

Introduction
Sewage sludge is a semi-solid waste generated from urban sewage treatment that contains high concentrations of pollutants such as heavy metals, pathogens, and organic compounds. It necessitates appropriate management, and how this sludge can properly be disposed of has become a critical environmental issue [1-3]. At present, there are three main methods for sludge disposal: chemical treatment (adding chemical components), thermal treatment (incineration, pyrolysis, gasification), and biological treatment (earthworm composting, composting, anaerobic digestion, autothermal thermal aerobic digester [3], and others). The three disposal methods have different advantages and disadvantages. Chemical treatment is simple to operate with minor nitrogen loss, but it is costly and increases the dry weight of residual sludge. Heat treatment takes a short time with a high weight reduction ability and the ability to recover carbon; however, it is technically complex, costly, and requires control of emitted gas pollutants [4]. Considering other factors such as cost and recycling capacity, biological disposal appears to be a suitable method for disposing of sludge [5].
Composting is a biological treatment method involving the controlled decomposition of organic waste under aerobic conditions through the use of the enzymatic activity of microorganisms [6, 7]. Recycling sludge compost for agricultural use and soil improvement is often one of the most convenient, effective, and cost-effective disposal options [1, 8]. During the composting process, harmful substances and pathogens in sludge can be eliminated, and nutrients such as nitrogen and phosphorus can be recovered and converted into organic fertilizers [9]. The physical and chemical properties of sludge are unsuitable for direct composting, meaning it can only be recycled into high-quality products through co-composting [10]. Many studies have added improved materials to sludge compost to achieve synergistic effects in stabilizing waste, and in recent years, significant achievements have been made in co-composting sludge with various additives to improve the quality and maturity of compost, such as rice husks, earthworms, biochar, and sawdust. [7, 8, 11, 12].
Research into earthworm composting began in the late 1970s and is considered an effective, environmentally friendly technology for treating sewage sludge [13]. Due to the complex composition of the initial sludge and the high-temperature environment formed during fermentation, it is often necessary to pre-compost the sludge when using earthworm composting to avoid killing the worms. To get around this issue, some scholars have shifted their focus from earthworm addition to adding only earthworm mucus, a lubricant secreted from the epidermis of earthworms that is mainly composed of water, lipids, carbohydrates, sugars, proteins, and amino acids [14, 15]. It plays a crucial role in earthworm movement, feeding, excretion, osmotic regulation, defense, and reproductive activities [16-18]. Bityutskii et al. have demonstrated that earthworm mucus in soil can drive the mineralization and humification of plant residues [19]. In addition, studies have also found that adding earthworm mucus to earthworm compost can change the bacterial community structure and accelerate the mineralization and humification of compost materials [20]. Although earthworm mucus has been proven to have significant utilization value, there have been no reports on the direct use of earthworm mucus in sludge composting, and it is necessary to explore whether the direct addition of earthworm mucus could positively affect the sludge composting process.
Decomposition by microorganisms plays a crucial role in the transformation and stability of organic matter (OM) during composting. Bacteria are one of the most important types of microorganisms, and understanding their community changes during composting is of great significance for understanding the overall process as well as the microbiological mechanisms involved. To date, scholars have explored the changes in microbial community structure in composting systems, however, most have used human or livestock manure as raw materials and biochar or microbial agents as additives. In addition, some scholars have studied the effect of earthworm mucus on sludge composting, but this study is based on earthworm composting [20].
There have been few reports on directly adding earthworm mucus to sludge compost and exploring the succession of bacterial communities that occur in response. Considering the potential utilization value brought by the complex components and special functions of earthworm mucus, this study evaluated the impact of earthworm mucus on sludge composting, especially the changes in bacterial composition that occur and their responses to environmental factors, to provide new directions for sludge resource utilization using this treatment method.
Materials and Methods
Test Materials
The municipal sludge used originated from a wastewater treatment plant in Huainan City, Anhui Province, China, with a moisture content after deep dewatering of 75-80%. The test sludge was fresh and was immediately transported back to the laboratory for composting testing after sampling. Earthworms produced the mucus used in the experiment after electrical stimulation at 5 V and 10 mA; the earthworms used were Taiping II Eisenia fetida purchased from the Jurong Earthworm Breeding Base in Jiangsu Province, China, commonly known as red earthworms. They had a fresh weight of ~0.5 g per worm. Each experimental material’s basic physical and chemical properties are shown below (Table 1). Analytical methods are described in Section 2.3.
Table 1.
Basic properties of test materials
Test Methods
The sludge was composted alone to establish a control (CK) with a total sludge weight of 4 kg, and 80 mL of earthworm mucus was added to the test group (M) [20], both of which were supplemented with approximately 200 g of rice husk to regulate the carbon to nitrogen ratio of the sludge. All treatments were set up in three parallel samples. The composted substrate was placed in a compost box with a length × width × height of 24 × 21 × 26 cm and was composted for 35 days. A compost box was used to control the temperature throughout the composting process, which was maintained at 40 °C on day 0, at 50 °C on days 1-8, and then decreased by 5 °C per day after day 9 until room temperature was reached. The box then entered a natural decay phase until the end of the composting process. During the first 15 days, the piles were turned twice a day and ventilated five times (at a rate of 0.5 L·min-1), then ventilated twice daily for the next 20 days and turned every 2 days.
Compost temperature (T) was measured in the morning and evening every day, and the average value was recorded as the temperature of the heap for that day. Samples were taken on days 0, 4, 8, 13, 19, 26, and 35, and around 150 g of samples were collected each time. Portions (10 g) of samples were stored in a refrigerator at 4 °C for the determination of physicochemical properties such as pH, EC, moisture content, and OM; 130 g were naturally air-dried for the determination of total nitrogen, total phosphorus, and total potassium; and 10 g were stored in a refrigerator at -80 °C for bacterial community analysis.
Physicochemical Parameter Analysis
Moisture content (MC) was determined by weight loss in an oven at 105 °C. pH and electrical conductivity (EC) were determined by a benchtop acidimeter (PHS- 3C, Shanghai Precision Scientific Instrument Co., Ltd., China) and a benchtop conductivity meter (DDS-307A, Shanghai Yidian Analytical Instrument Co., Ltd., China), respectively, using the methods reported by Jining et al. [21]. Total nitrogen (TN) and total phosphorus (TP) were determined using the alkaline potassium persulfate digestion-UV spectrophotometric method and the ammonium molybdate spectrophotometric method, respectively (N4S, Shanghai Yidian Analytical Instruments Co., Ltd., China), and total potassium (TK) was determined by an inductively coupled plasma-optical emission spectrometer (Avio 550 Max, PerkinElmer Corporate Management (Shanghai) Co., Ltd., China) [22]. The OM was determined by drying the samples in an oven at 105 °C and then burning them in a muffle furnace at 550 °C until they reached a constant weight [23].
DNA Extraction and PCR Amplification
Microbial DNA was extracted from mouse feces specimens using the FastLee DNA kit for Feces (Hangzhou Legenomics Bio-Pharm Technology Co., Ltd., Hangzhou, China) according to the manufacturer’s instructions. The V3-V4 region of the bacteria 16S ribosomal RNA gene was amplified by PCR (95 °C for 2 min, followed by 25 cycles at 95 °C for 30 s, 55 °C for 30 s, and 72 °C for 30 s, and a final extension at 72 °C for 5 min) using primers 341 F 5ʹ-barcode- CCTAYGGGRBGCASCAG)-3ʹ and 806 R 5ʹ-GGACTACNNGGGTATCTAAT-3ʹ, where the barcode was an eight-base sequence unique to each sample. The PCR reactions were performed in triplicate with 4 μL of 5X FastPfu Buffer, 2 μL of 2.5 mM dNTPs, 0.8 μL of forward primer (5 μM), 0.8 μL of reverse primer (5 μM), 0.4 μL of FastPfu Polymerase, 0.2 μL of BSA, and 10 ng of template DNA, topped up with ddH2O to a final volume of 20 μL. Amplicons were extracted from 2% agarose gels and purified using the AxyPrep DNA Gel Extraction Kit (Axygen Biosciences, Union City, CA, U.S.) according to the manufacturer’s instructions and quantified using QuantiFluor™-ST (Promega, U.S.).
Data Processing and Analysis
Raw data processing and analysis were done using Excel 2021 and SPSS24. One-way analysis of variance (ANOVA) and least significant difference (LSD) were used to analyze the physicochemical properties as well as microbial community structure in the compost samples; physicochemical parameters and microbial abundance were plotted using Origin 2022. Redundancy analysis (RDA) plots were plotted via the Parnassian Genome Cloud platform (https://www.genescloud.cn). The significance was set at 0.05 and 0.01.
Results and Discussion
Changes in Physicochemical Parameters During Composting
Analysis of Physical Indicators
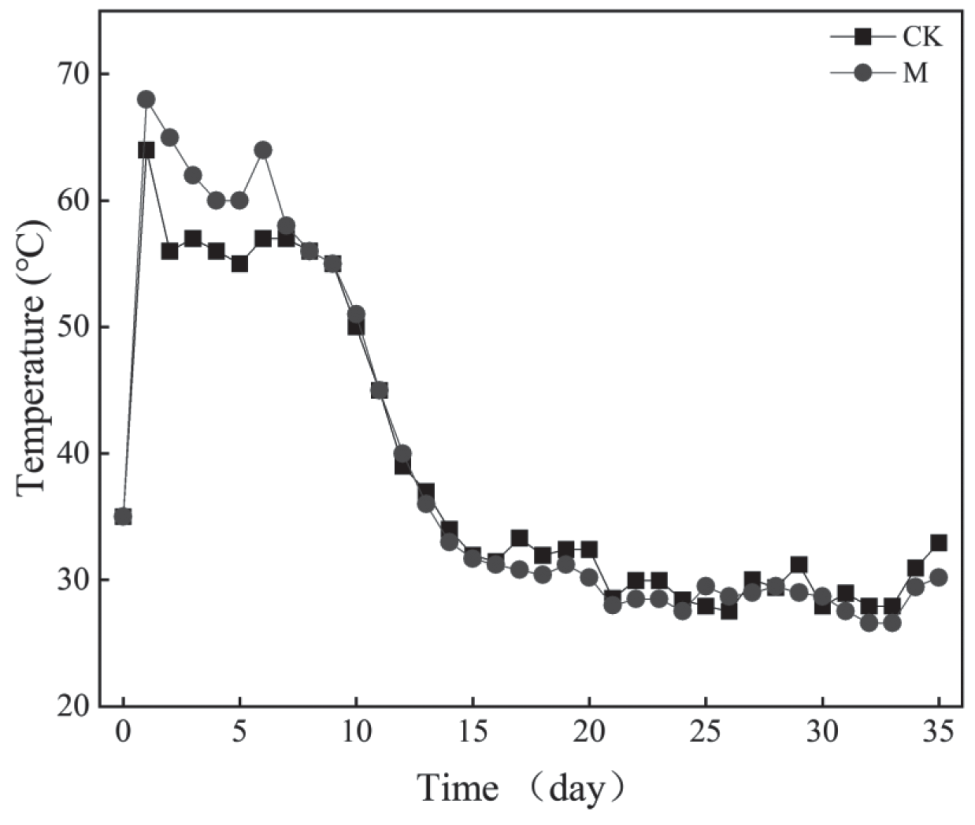
Temperature is one of the critical parameters in composting and is key in evaluating the composting process [7, 24]. As shown in Figure 1, the compost temperature of both the CK and M treatments first increased before decreasing and then stabilizing, corresponding to four phases: heating, high-temperature, cooling, and maturation periods. The CK treatment only remained in the high-temperature period of ≥ 60 ℃ for one day, while the M treatment remained in this phase for six days. The CK and M treatments entered the high-temperature period on the first day of the reaction and reached their highest temperatures of 64 and 68 ℃, respectively. The M treatment heated up faster than the CK treatment, and during the entire high-temperature period, the temperature of the M treatment was significantly higher than that of the CK treatment. This indicated that adding earthworm mucus increased the temperature during sludge composting and prolonged the high-temperature period. This is likely because earthworm mucus can provide a suitable living environment and necessary materials for microbial activity, resulting in higher microbial abundance and metabolic activity in the M treatment and affecting the heating and high-temperature periods [20, 25]. In addition, thermophilic microorganisms have higher metabolic activity during the high-temperature period and continue to produce heat to maintain high temperatures [26]. In the later stage of composting, with the consumption of easily degradable OM, the substances required by microorganisms decreased, leading to decreased metabolic activity. As a result, the temperature gradually decreases, and the compost enters the maturation stage.
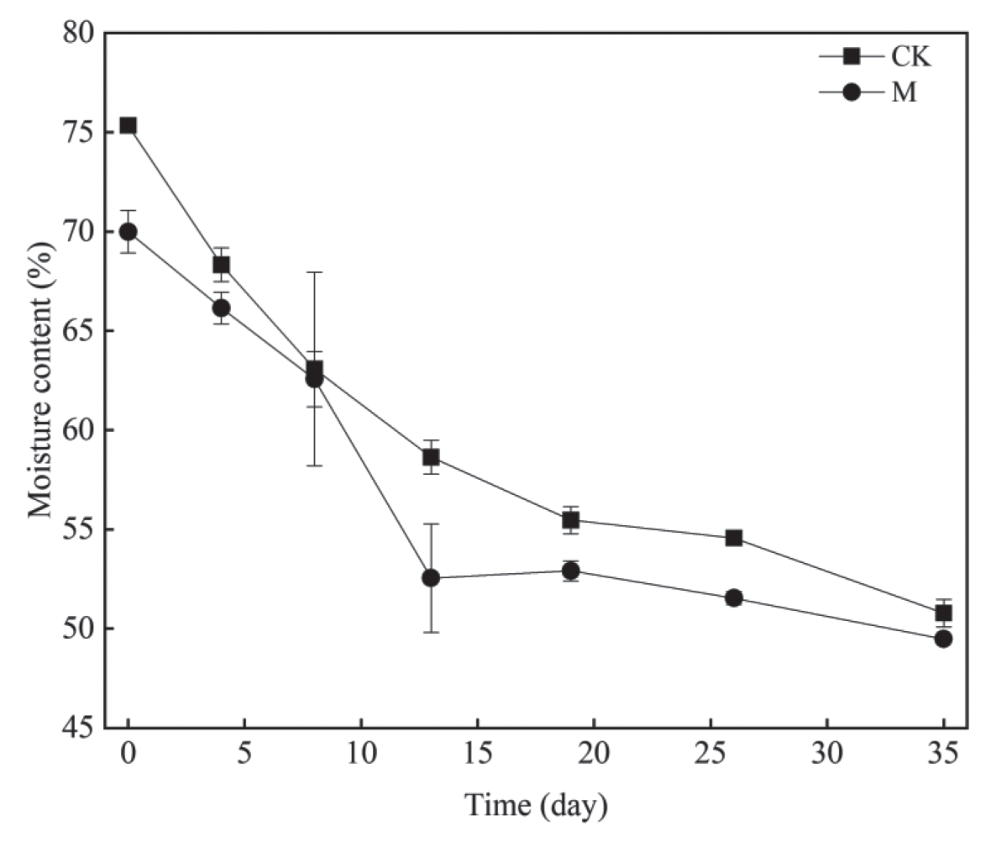
Changes in MC significantly impact the composting process. Appropriate moisture content provides suitable environmental conditions to promote microbial activity and facilitate OM decomposition. Excessive or insufficient moisture can affect the stability of the composting process and the decomposition rate of OM [27, 28]. The moisture content of the sludge in both treatments gradually decreased (Figure 2). During the heating and high-temperature stages (0-13 days), the moisture content of sludge in the CK and M treatments rapidly decreased by 22.18 and 24.91%, respectively. During days 0-8, this may have been due to the initial moisture content of the sludge in the CK treatment being too saturated, resulting in a faster decrease than in the M treatment. After the eighth day, the rate of moisture content decrease in the M treatment was significantly higher than that in the CK treatment, mainly because of the higher activity and abundance of microorganisms in the M treatment and higher water consumption and volatilization. After composting, the moisture content of the sludge in the CK and M treatments remained stable at around 50% (50.78 and 49.47%, respectively), meeting the standard (< 65%) stipulated in the Chinese Urban Wastewater Treatment Plant Pollutant Discharge Standard (GB18918-2002).
Analysis of Chemical Indicators
pH is an important indicator affecting microbial activity during composting; too high or too low pH can severely impact microbial growth and activity. Composting requires a neutral or slightly alkaline environment [29]. As shown in Table 2, the pH values of both CK and M treatments rapidly increased in the early stage and remained stable after reaching high values on the eighth day. The entire composting process remained in a slightly alkaline environment. The early increase in pH value was mainly due to the degradation of nitrogen-containing substances and the accumulation of NH4+-N in composted sludge [30]. The reduction of degradable substances in the later stage led to weakened ammonification, which, combined with the conversion of NH4+-N through nitrification or assimilation [31], maintained a stable pH.
Changes in OM and EC can reflect the degree of OM degradation and transformation in the reactor and are also important indicators for evaluating whether sludge composting can be applied. According to Table 2, the changes in OM content in the two treatments were opposite to those seen in pH. As composting progresses, the OM in the sludge continuously degrades, resulting in a continuous decrease in OM content. The trend of EC value change corresponds to the change in OM content; before entering the maturation period, the rapid degradation of OM and the release of a large number of water-soluble minerals leads to a continual EC value increase [32], while the decrease in OM degradation in the later stage keeps the EC value stable. Comparing the CK treatment with the M treatment, the degradation efficiency of OM in the M treatment reached 19.35%, significantly higher than the 13.91% seen in the CK treatment; the degradation rate of OM in the M treatment was higher than that in the CK treatment during the high-temperature period. This is because the earthworm mucus added to the M treatment enhanced microbial activity, initiating OM mineralization and humification and accelerating the decomposition of OM [19]. Adding earthworm mucus to sludge compost was found to be beneficial for OM degradation, improving the effectiveness of sludge composting.
Nutrient Analysis
The changes in TN, TP, and TK in compost under different treatments are shown in Table 2. During the initial 0-4 day high-temperature period, the TN content of the CK treatment rapidly decreased and stabilized, showing an overall decreasing trend, while the M treatment’s TN content remained stable throughout the composting process. Although microorganisms decompose a large amount of nitrogen-containing OM during composting [33], resulting in a decrease in TN, the microbial activity and abundance in the M treatment were higher than those in the CK treatment. The maturity and dry matter loss were also higher, leading to a more significant concentration effect [30]; as a result, the TN content in the compost increased, offsetting loss through biodegradation and making the TN content in the M treatment remain relatively stable. In the middle and later stages of composting, the TN content in both the CK and M treatments stabilized due to the slowing of the consumption and concentration effects of degradable nitrogen substances.
During the entire composting process, the TP content fluctuated in both treatments. After composting, the TP content in the CK treatment slightly decreased, while the TP content in the M treatment increased by 12.13%. Studies indicate that this increase in TP content may be due to OM mineralization [13]. Another study on earthworm composting found increased TP content, suggesting that the phosphorus-solubilizing microorganisms (PSB) present in the earthworm gut may release phosphorus from organic phosphates [34, 35].
Unlike nitrogen and phosphorus, potassium showed a clear upward trend during composting, with an initial increase followed by a decrease. The TK content in both CK and M treatments reached its maximum on the eighth day (14.71 and 14.36 g·kg-1, respectively), gradually decreasing after that. At the end of composting, the TK content in the M treatment increased by 24.45%, much higher than the 14.22% increase seen in the CK treatment. This is because microorganisms produce more small-molecule organic acids that can dissolve a portion of insoluble potassium that then enters the compost. The addition of earthworm mucus enhanced microbial activity, so it exacerbated this effect, resulting in a significant increase in TK content in the M treatment compared to the CK treatment [13, 36].
Table 2.
Physicochemical indicators of compost samples at different stages of composting
Nitrogen, phosphorus, and potassium, as nutrients in composting systems, significantly impact the subsequent utilization of compost products. It can be inferred from the results that adding earthworm mucus to compost sludge is an effective means to promote the resource utilization of sludge, which is reflected in the reduced nitrogen loss and increased content of phosphorus and potassium.
Changes in Bacterial Community Diversity During Composting
Changes in Bacterial Diversity Indices
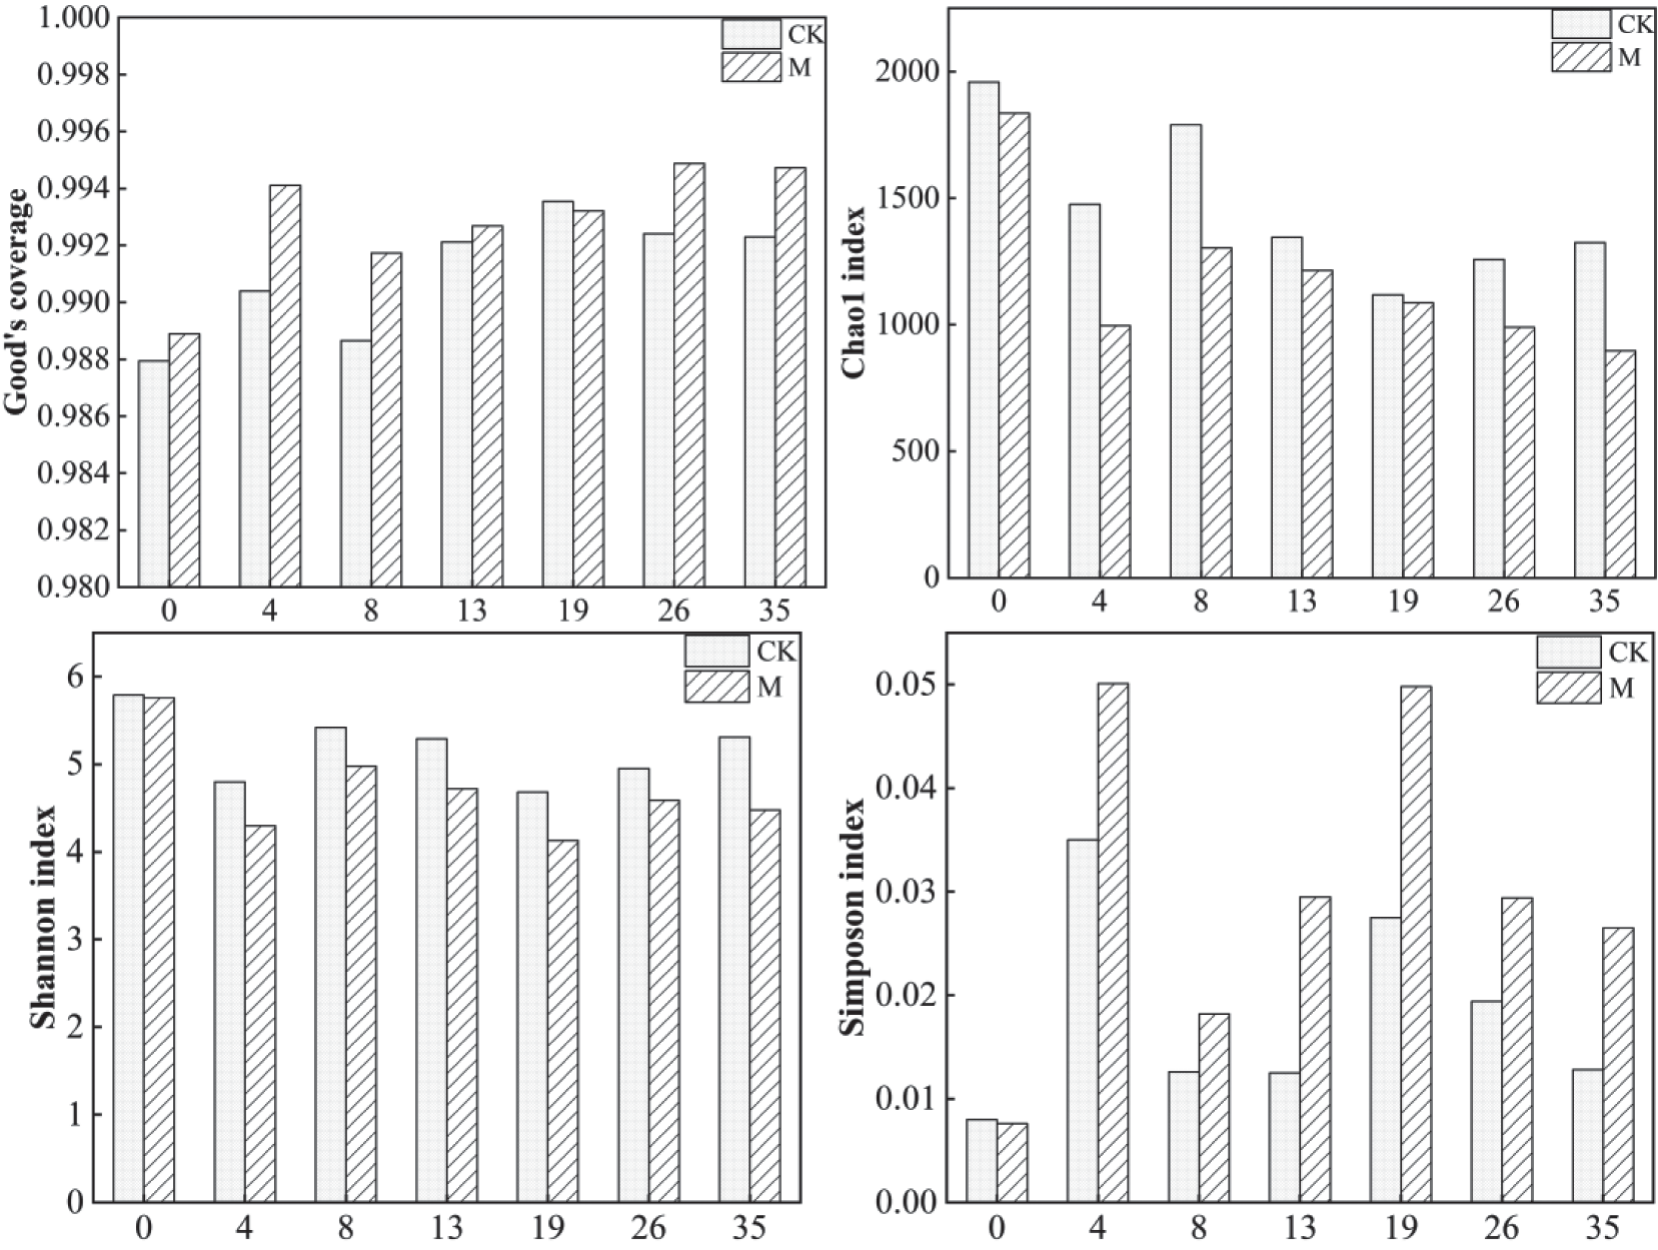
Good’s coverage represents the coverage of all sample libraries, with a larger value indicating higher coverage by the obtained sequences (Figure 3). The coverage indices of each stage of the two composting experiments exceeded 98.79%, indicating that the results accurately reflected the actual community of bacteria in the samples [37]. The Chao1 index is an indicator of ecosystem species diversity [32]. As composting proceeded, the Chao1 index in both CK and M treatments first decreased, then increased, then decreased again (Figure 3). The Chao1 index of sludge composting alone (CK) was always higher than that of composting with added mucus (M); specifically, the Chao1 index of composting rapidly decreased during the high-temperature period and then increased again after 5-8 days before gradually decreasing until the end of composting. The Shannon index is based on species richness and evenness, considering changes in species quantity and relative abundance; the higher the index, the higher the species richness and evenness in the sample and the richer the biodiversity [23]. Simpson’s index is based on species richness, which measures the relative abundance of a species in a sample; the lower the index, the higher the species richness and biodiversity in the sample. As shown in Figure 3, the changes in these two indices in the CK and M treatments reflected the same pattern of bacterial diversity changes as the Chao1 index. Bacterial diversity decreased from days 0-4 days, increased again within 5-8 days, and finally slowly decreased and tended to stabilize. This is because the rapid increase in temperature during the early stage of composting was difficult for some bacteria to adapt to, leading to a large amount of bacterial death [38], and resulting in a decrease in bacterial diversity. During the 5-8 day reaction phase, the temperature decreased slightly, and a large number of thermophilic bacteria adapted and rapidly began to reproduce, leading to an increase in bacterial diversity. In the later stage of composting, as easily degradable OM continued to be consumed, the competitiveness between microorganisms increased, and bacterial activity and diversity continued to decline. The bacterial diversity in the CK treatment was higher than in the M treatment during composting, mainly for two reasons: firstly, the more drastic temperature changes in the M treatment led to more bacteria not adapting and dying, and secondly, the addition of earthworm mucus promoted the growth of dominant bacterial communities, intensifying competition for resources [39,40], resulting in the rapid disappearance of disadvantaged bacterial communities. Because of this, bacterial diversity was lower in the CK treatment.
Changes in Bacterial Community Structure at the Phylum and Genus Levels
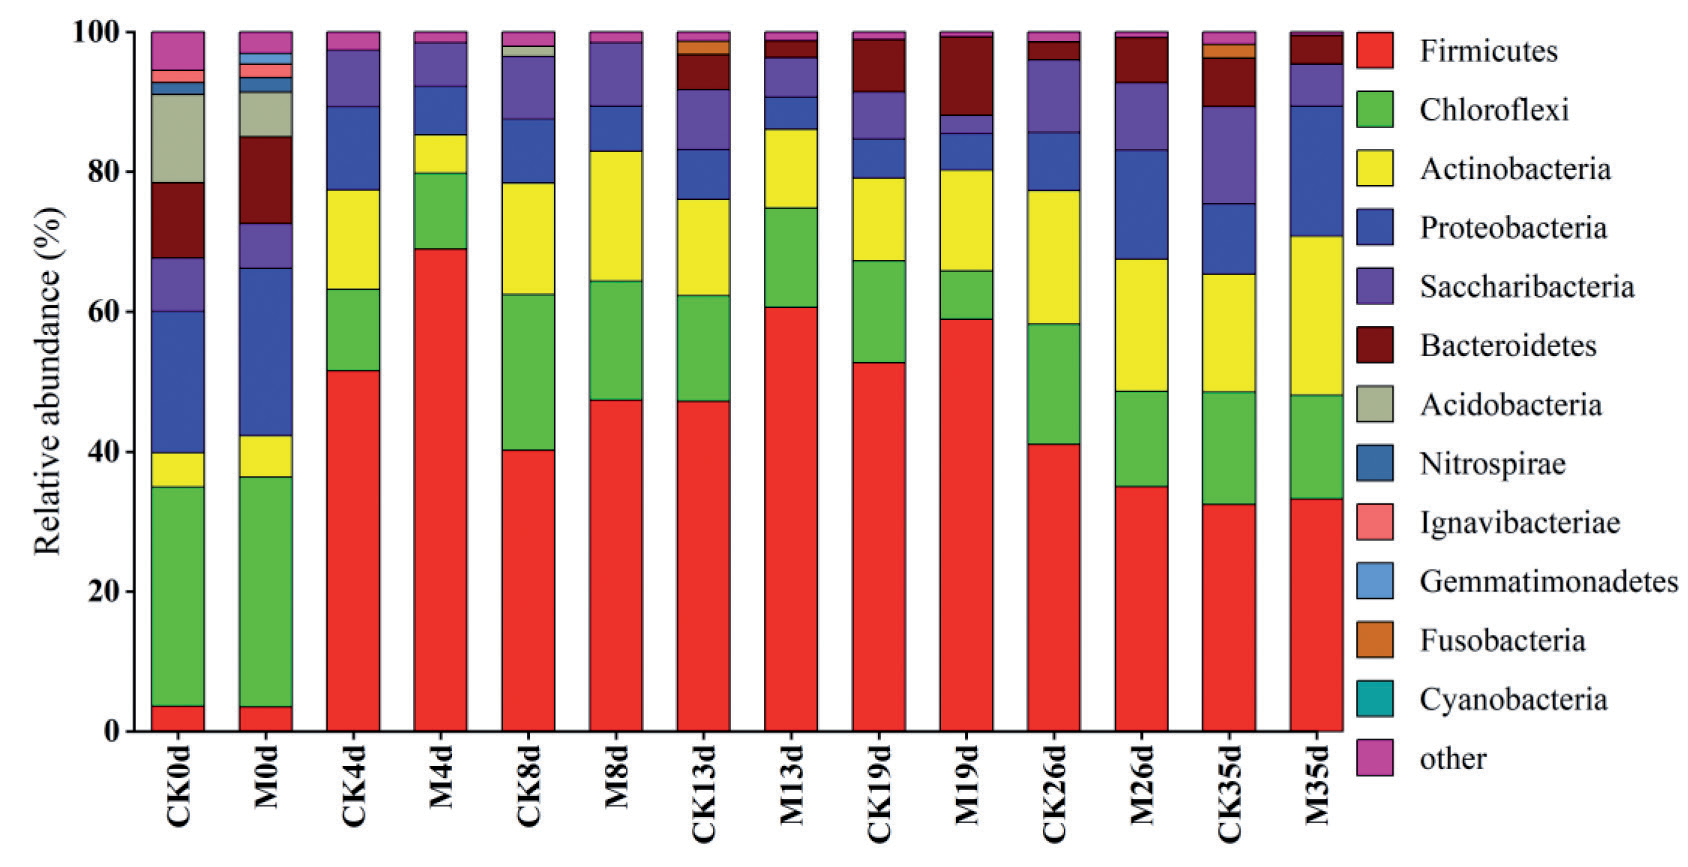
Figure 4 shows the horizontal distribution of microbial community structure during composting. On day 0, the CK and M treatments were both mainly composed of Firmicutes, Chloroflexi, Actinobacteria, Proteobacteria, Saccharibacteria, Bacteroidetes, and Acidobacteria as the dominant bacterial phyla. This is similar to the results of Xin et al. examining co-composting waste mushroom substrates, chicken manure, and Chinese medicine residues [41]. In addition, Yi et al. reported that after inoculating thermophilic nitrifying bacteria during sludge composting, Actinobacteria, Firmicutes, Proteobacteria, and Chloroflexi dominated the composting process.
When composting entered the high-temperature period, the temperatures of the two treatment groups rapidly increased, and the relative abundance of each bacterial phylum changed. The number of dominant bacterial phyla also decreased, but Firmicutes, Chloroflexi, Actinobacteria, Proteobacteria, and Saccharibacteria remained dominant, with a total relative abundance exceeding 96%. The relative abundance of Firmicutes rapidly increased to > 40%, becoming the most dominant phylum. Firmicutes are widely present during the thermophilic period of composting as they can produce spores to withstand high temperatures [42]. Chloroflexi and Proteobacteria relative abundance rapidly decreased after composting began, contrary to the results reported by Zhicheng et al. [22], which may be related to the intense competition between dominant bacteria. The abundance of Actinobacteria slightly increased from the high-temperature period to the maturation stage, mainly due to its ability to degrade complex organic compounds such as cellulose and lignin as well as its role in carbon and nitrogen conversion [43, 44]. After the high-temperature period until the end of composting, Bacteroidetes became one of the dominant phyla, while other dominant phyla remained unchanged. This phylum is crucial for the utilization of lignocellulose and the subsequent release of short-chain fatty acids, explaining their increasing relative abundance during the composting stage [45]. The relative abundance of dominant bacteria in the M treatment with the ability to degrade complex OM, such as lignin and cellulose, was higher than that in the CK treatment from the beginning of the composting process until maturity (0-18 days), indicating that adding earthworm mucus improved the composting efficacy.
To further explore the microbial community structure of composting, the horizontal distribution of bacterial genera was analyzed (Figure 5). During composting, the main dominant bacterial genera were Bacillus, Caldicoprobacter, Saccharibacteria_Norank, Tepidimimicrobium, and Ureibacillus. In the early stage of composting (0 days), the dominant bacterial genera for CK and M treatments were Anaerolineaceae_Uncultured, Caldilineaceae_Uncultured, Saccharibacteria_Norank, Saprospiraceae_Uncultured, and TK10_Norank. When composting entered the high-temperature period, the horizontal distribution of bacterial genera underwent drastic changes, with Bacillus, Caldicoprobacter, and Saccharibacteria_Norank, Tepidimimicrobium, and Ureibacillus becoming the dominant bacterial genera in both treatment groups, with the total combined relative abundance reaching 47.49 and 58.86% for CK and M treatments, respectively, on the fourth day. As the compost continued to ferment and mature, the main dominant bacterial genera remained unchanged, but their relative abundance fluctuated. At the end of composting (26-35 days), significant changes occurred in the dominant bacterial genera in both treatment groups, with Bacillus, JG30-KF-CM45_Norank, Micromonosporae_ Unclassified, Ureibacillus, and Saccharibacteria_Norank being the dominant bacterial genera in the CK treatment, while the dominant bacterial genera in the M treatment now included Pusillimonas and Rhodococcus.
Compared with the CK treatment, the M treatment with added mucus showed a higher trend in the abundance of dominant bacterial genera throughout the entire composting process, mainly reflected in both Bacillus and Ureibacillus. Bacillus and Ureibacillus are the prominent representatives of Firmicutes, which are widely present bacterial community components during the composting stage. According to reports, Bacillus mainly survives in compost by forming endophytic spores that can tolerate high temperatures [46]. In addition, studies have shown that Bacillus can compete with other microorganisms because of its antifungal and protease activities [47, 48]. Rong et al. reported that Ureibacillus is an aerobic thermophilic bacterium that can degrade lignocellulose [49]. Adding earthworm mucus resulted in a more efficient macromolecular degradation system in the M treatment.
Relationship Between Environmental Factors and Changes in Bacterial Communities
Changes in bacterial communities can significantly impact the composting process, especially its efficacy. Studies have reported that bacterial community succession is driven by changes in environmental conditions and substrate composition at each composting stage [50]. Understanding the impact of environmental factor changes during composting on microbial community succession is particularly important. The influence of environmental factors on the relative abundance of the top six phyla in earthworm mucus compost sludge was analyzed using RDA. As shown in Figure 6, the RDA1 and RDA2 axes explained 68.01 and 3.43% of the changes in bacterial community structure and environmental factors, respectively. Together, the two axes explained 71.44% of the sample information, indicating that physical and chemical factors are related to changes in bacterial community structure during composting. At the phylum level, the correlation order between environmental factors and bacterial community structure was EC>MC>pH>OM>TN>T, but the difference is minimal. Specifically, T, pH, and EC were positively correlated with Firmicutes, Actinobacteria, and Saccharibacteria but negatively correlated with Chloroflexi and Proteobacteria; MC, TN, and OM were positively correlated with Chloroflexi and Proteobacteria, and negatively correlated with Firmicutes, Actinobacteria, and Saccharibacteria.
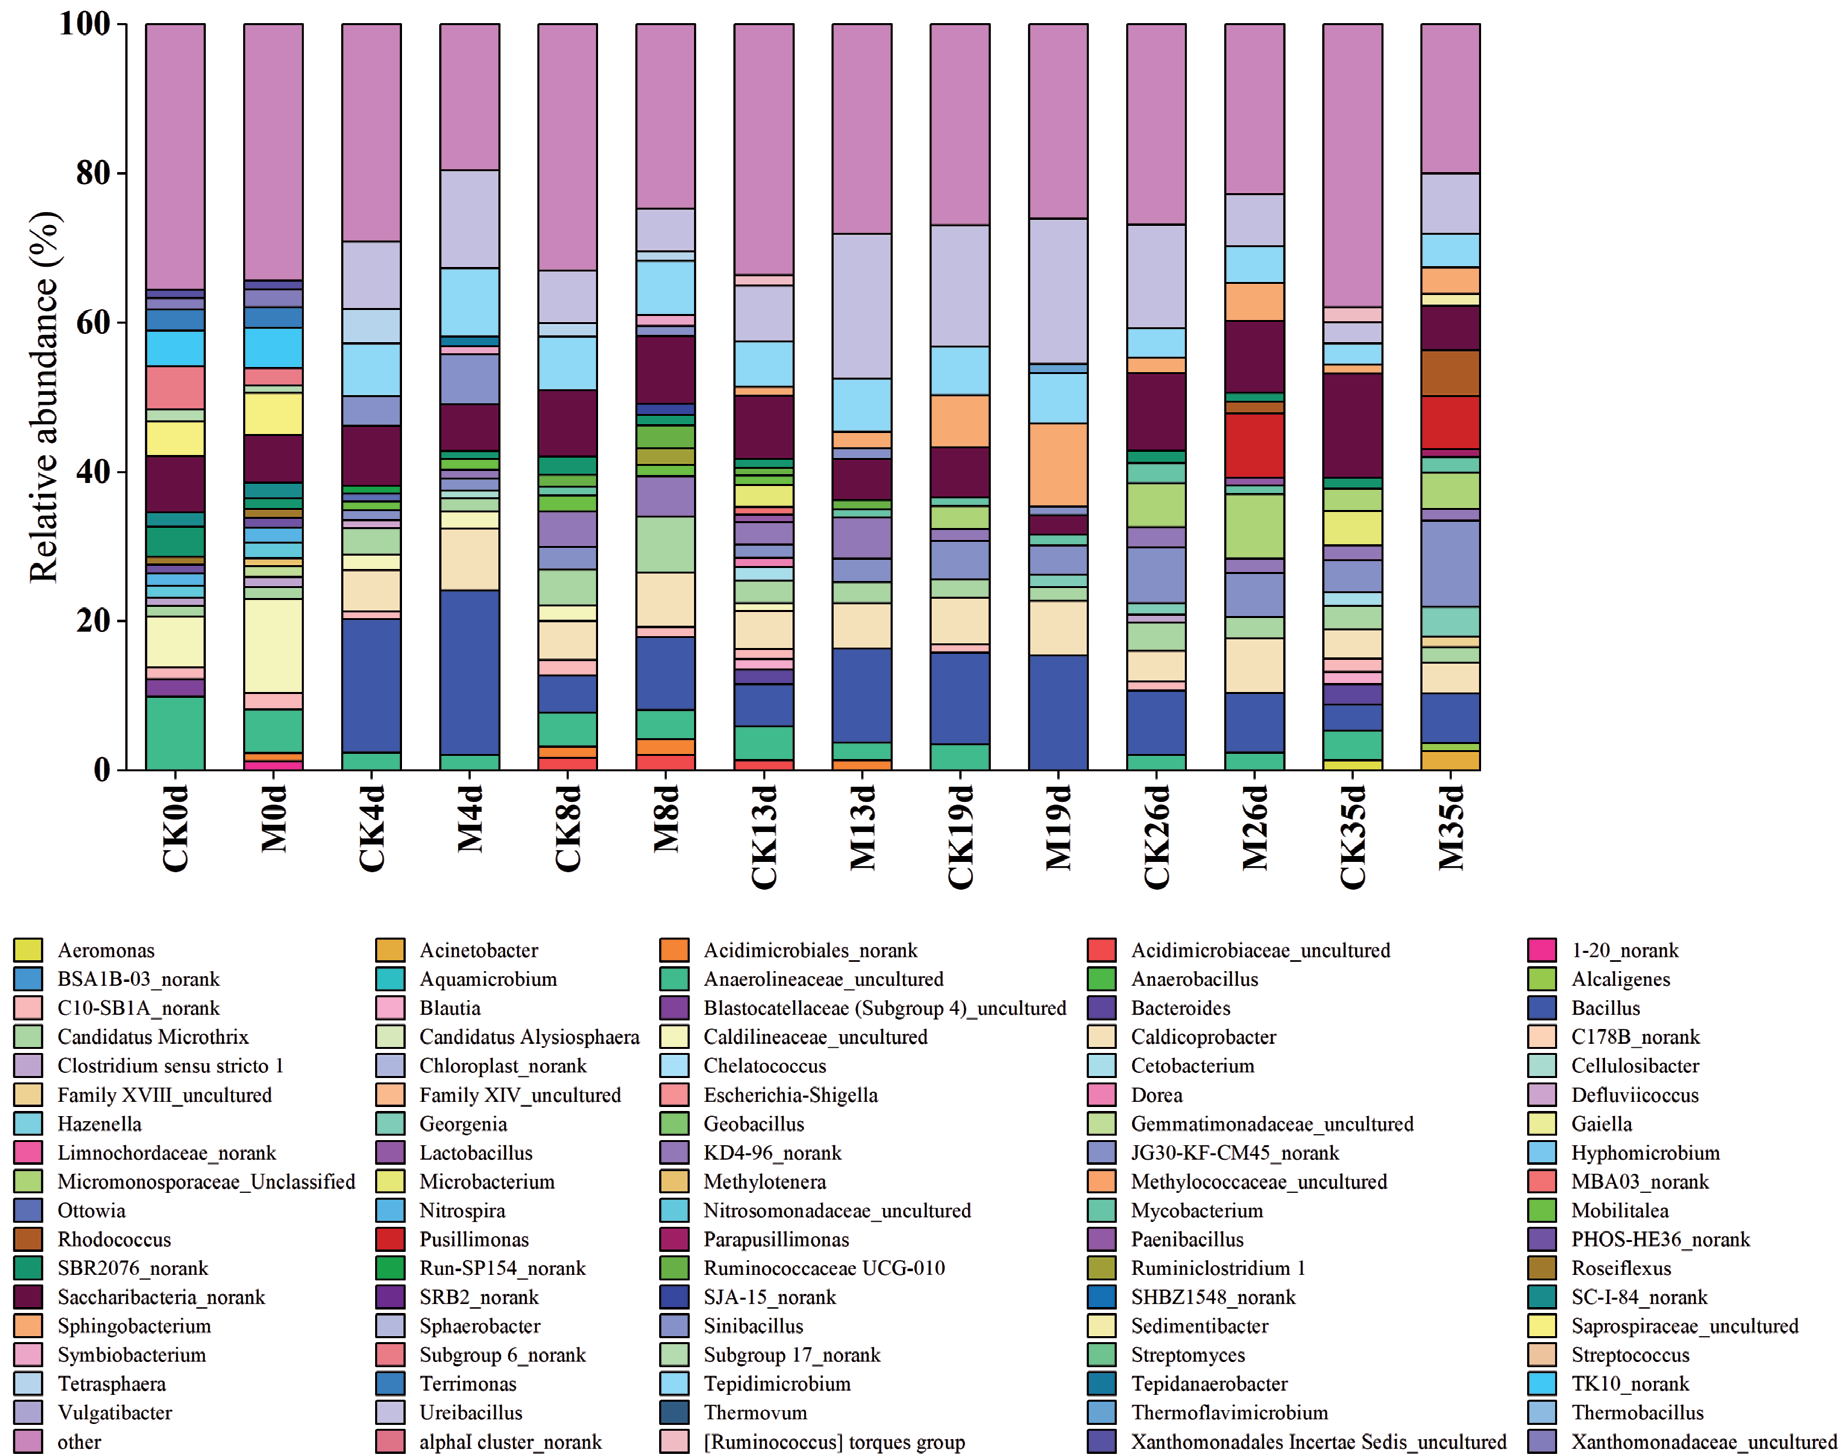
Fig. 6.
Redundancy analysis of environmental factors and bacterial community structure during composting (gate level). The arrow length in the RDA graph represents the degree of correlation between environmental factors and sample distribution.
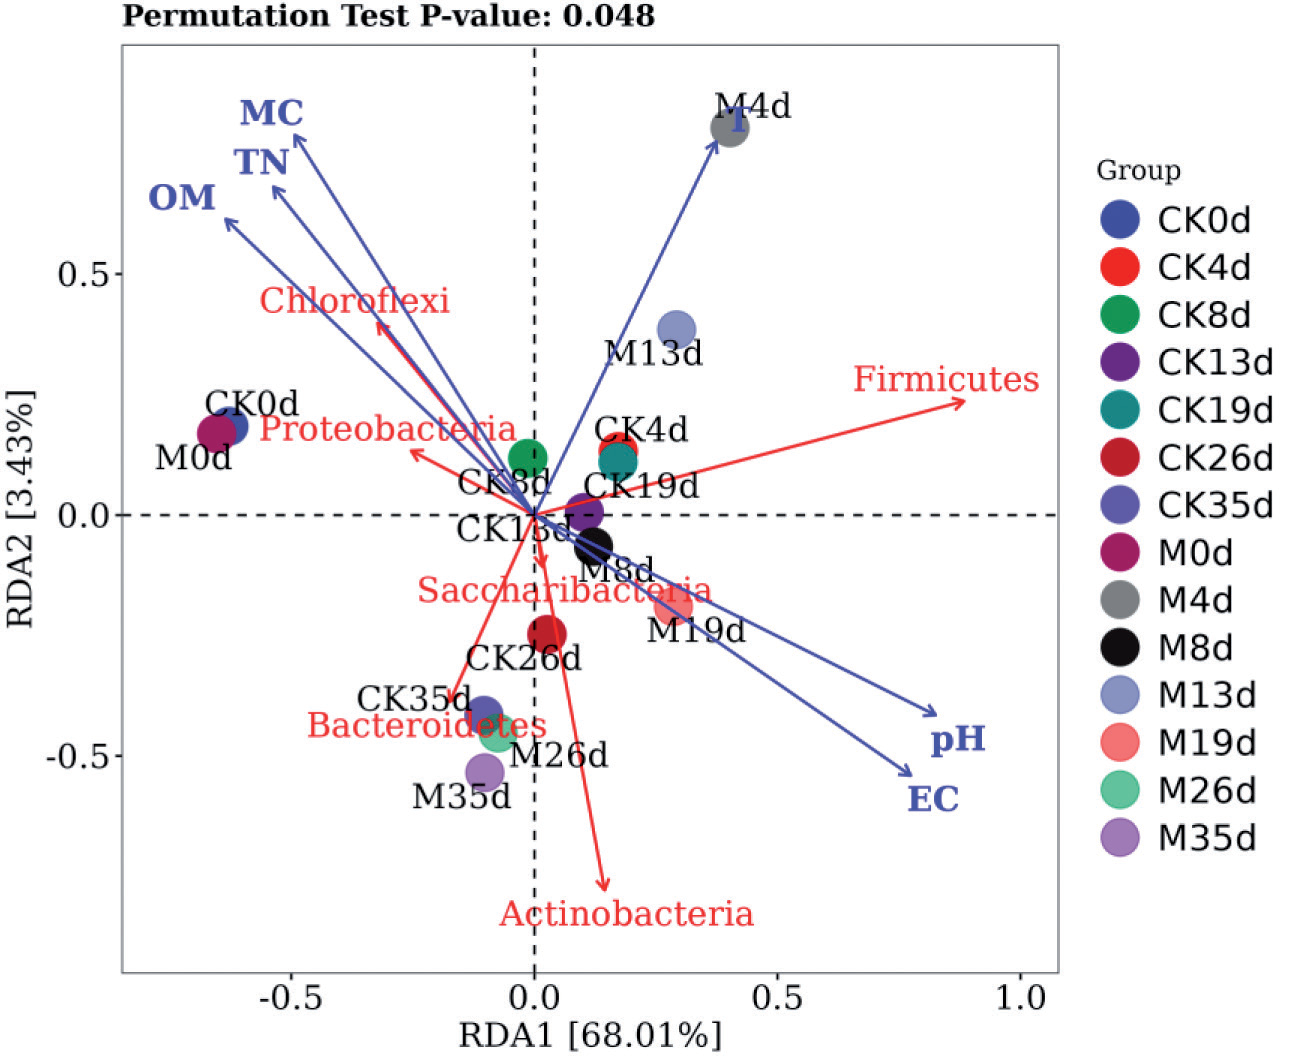
Although the impact of T on bacterial communities in this study is relatively small compared to other environmental factors, it has been reported that it is still an essential factor affecting microbial metabolism during composting [22, 42, 51]. Both high and low pH can seriously impact microbial activities. Lucas et al.’s research suggests that changes in pH can lead to changes in nutrient availability, such as calcium and magnesium, which may indirectly affect bacterial communities [52]. For this study, the above conclusions are directly reflected in the Firmicutes phylum, which had the highest relative abundance during the composting process, and pH was the environmental factor with the strongest positive correlation during the thermophilic stage. For Actinobacteria, which play a vital role in the decomposition of lignocellulose, the most negatively correlated environmental factor was MC. According to reports, Actinobacteria can survive in harsh environments, such as those with high temperatures and reduced water content, by forming spores [53, 54]. In this study, the MC content in the M treatment during the thermophilic stage was lower than that in the CK treatment, and correspondingly, the relative abundance of Actinobacteria was higher in MC. TN and OM were the environmental factors with the strongest positive correlation with Chloroflexi and Proteobacteria, respectively, indicating that the nutrient content (C, N) in compost changed with the continuous transformation of microbial metabolites [54]. The results indicate that appropriately increasing pH and reducing MC during the high-temperature composting period could promote composting humification. Environmental factors (T, pH, MC, OM, TN, EC) in composting played a large role in the succession of bacterial community structure, as all kinds of bacteria are affected by environmental factors to different degrees. Regulating these environmental factors in the composting process may be an effective optimization method, especially in terms of improving bacterial community structure.
Conclusions
This study examined the addition of earthworm mucus to composting sludge to determine its effects on composting efficacy and the microbial community involved. The addition of earthworm mucus optimized sludge composting and played a prominent role in reducing nitrogen loss and increasing nutrients. Earthworm mucus increased the relative abundance of dominant bacteria in sludge compost, which is beneficial for sludge maturation. Environmental factors significantly impacted the bacterial community structure during sludge composting. These results indicate that sludge composting can be optimized for improved efficacy by regulating environmental factors.

