

Introduction
As important components of forest soil and ecosystems, microorganisms play important roles in soil formation, organic matter synthesis and decomposition, material transformation and energy transfer of forest ecosystems [1-3]. Soil microorganisms are the main decomposers in forest ecosystems and the main determinants for plant health. As the nutrition and energy sources of soil microorganisms, the secretions produced by plant roots indirectly affect soil microbial diversity by changing soil nutrients and structure [4-7]. Biological and abiotic factors in forest soil affect the growth and development of trees greatly, in contrast, the tree species and their growth and development process also affect the soil microbial community structure [8]. Among the soil microbial community, bacteria and fungi predominate and play key roles in material cycle and energy flow in the forest ecosystem, which are also important indicators because of its sensitivity and activity to environmental change [9]. Bacteria is the most abundant and diverse microbial group in rhizosphere soil, some kinds of bacteria promoted the growth and development of plants, and some of the others inhibited [10]. The soil fungi could promote the nutrients absorption by host plants, improve plant resistance, change the bacterial community in soil, improve soil fertility, and decompose toxic substances in soil [11]. Moreover, some of fungi could form a symbiotic relationship with tree roots, and then promote trees growth, improve trees resistance to biotic and abiotic stresses [12, 13].
The physical and chemical characteristics of soil affect the types and distribution of microbial communities in soil microenvironment. In the soil, microbial communities between rhizosphere and non-rhizosphere differed in physical and chemical characteristics. The rhizosphere soil is a micro area constructed by complex interactions between host plants and the beneficial or harmful microorganisms, which contains abundant microbial resources and is influenced readily by plant roots. Changes of the physical and chemical characteristics of soil would affect the microenvironment where microorganisms lived, and then affect the species, activity and distribution of soil microbial communities [14]. Recently, the interaction between soil microorganisms and plant growth were studied by using molecular biology methods such as microbiology, proteomics, transcriptomics and Miseq sequencing technology [15], which can reveal the community structure and diversity relationship between forest soil in rhizosphere and non-rhizosphere at molecular level.
Juglans mandshurica (Manchurian walnut) is a Tertiary relict species in the Family Jugladandaceae, which is known as one of the “three hard broad tree species” together with Fraxinus mandshurica and Phellodendron amurense in northeast China forest region [16]. In recent years, J. mandshurica has been listed as a national Class II rare and endangered tree species because of decreasing natural forest caused by excessive logging. Currently, the research on J. mandshurica mainly focuses on the distribution of stands [17], the diversity of understory plants [18, 19], the species composition and diversity of secondary forests [20], the growth of seedlings [21], the physiological characteristics [22, 23], the selection of superior trees in natural forests and the diversity of fruits [24], reproductive biology [25, 26], the metabolism of substances for flower bud development [27] and chemical substances [28-30]. Sun et al. studied the juglone (the main substrate that caused self-toxic effect) concentration and soil microbial community structure in J. mandshurica plantations by detecting phospholipid fatty acid (PLFA) contents [31]. Their results indicated that large quantity of juglone were released into the rhizosphere soil, but little in non-rhizosphere soil. Further studies suggested that soil microbes (especially Gram-negative bacterium) facilitated juglone decomposition, while juglone inhibited the growth of soil microbes [32]. However, the research didn’t analyze the effects of soil physical or chemical characteristics on soil microbe, and they didn’t refine the species of the microbes.
In this study, the physical and chemical characteristics and the microorganism species and diversity in rhizosphere and non-rhizosphere soil in artificial demonstration forest of J. mandshurica were analyzed. The results will reveal the soil physical and chemical characteristics and the spatial differences of microbial distribution in rhizosphere and non-rhizosphere soil in the J. mandshurica artificial forest. Moreover, the relationship between soil microenvironment changes and microbial diversity were also clarified. These results will provide the theoretical and scientific basis for artificial cultivation and management of J. mandshurica large diameter timber.
Materials and Methods
Site Description
The study site located in Three Stone Forest Grounds of Fushun County (124°21′ 42″E, 41°45′32″N), Liaoning Province, where the J. mandshurica artificial demonstration forest was established in 2017. This area has obvious temperate continental monsoon climate characteristics and the soil type is dark brown forest soil. The annual maximum and minimum temperature are 38ºC and -33ºC, the average temperature is 6.04ºC, the average annual precipitation is 88.64 mm, and the frost free period is 145 d.
Experimental Design and Sampling
Three 15 m × 15 m sampling plots with spacing greater than 50m are set in the study area in early May 2020. Rhizosphere soil attached to the main root (less than 1 cm in diameter) at the depth of 10-30 cm (under the base of the tree trunk) is collected from 3-5 young J. mandshurica trees with similar growth characteristics randomly; and the non rhizosphere soil was collected randomly along a S-shape route at 10 sampling sites, where the soil were sampled using sterilized ring knife and mixed together after removing the topsoil. Rhizosphere and non-rhizosphere soil were put into the sterilized self sealing bag and then stored in the ice box immediately for soil microbial measurement. Soil samples used for soil bulk density (SBD) test were collected with an unsterilized ring knife at the 10 sampling sites. Soil samples used for chemical properties test were also collected at the 10 sampling sites with a shovel, about 2 kg of fresh soil was obtained after mixing the soil using the "quartering method". The fresh soil were then taken back for air drying, impurity removal, grinding and screening before chemical properties was determined.
Determination of Soil Physical and Chemical Characteristics
SBD was determined by ring knife method; soil pH was determined by pH meter; the total carbon (TC), total nitrogen (TN) and available nitrogen (AN) contents were determined by element analyzer; the total phosphorus (TP) contents were determined by H2SO4-HClO4 acid dissolution method; and the available phosphorus (AP) contents were determined by NH4F-HCl method. All tests were repeated three times.
Bacterial and Fungal Community Assessment
DNA Extraction and PCR Amplification
Microbial DNA was extracted using MO BIO Soil DNA Kits (MO BIO Laboratories, Carlsbad, CA, USA). The 16S rDNA V4-V5 region of the ribosomal RNA gene was amplified using primers 515F: 5’-GTGCCAGCMGCCGCGGTAA-3’, 909R: 5’- CCCCGYCAATTCMTTTRAGT-3’. The PCR amplification included: initial denaturation at 94ºC for 3 min , followed by 30 cycles of 94ºC for 40 s, 56ºC for 60 s, and 72ºC for 60 s, and a final extension at 72ºC for 10 min. The ITS rDNA region of the ribosomal RNA gene was amplified using primers ITS4: 5'- TCCTCCGCTTATTGATATGC-3' and gITS7F: 5'-GTGARTCATCGARTCTTTG-3'. The PCR amplification included: initial denaturation at 94ºC for 5 min, followed by 34 cycles of 94ºC for 30 s, 56ºC for 30 s, and 68ºC for 45 s, and a final extension at 72ºC for 10 min. PCR reactions were conducted twice for each sample, and the two PCR products for each sample were mixed together for agarose electrophoresis with a concentration of 1%.
Illumina Novaseq PE250 Sequencing
The target strips of agarose electrophoresis were recovered with DNA Gel Extraction Kit provided by Qingke, and the concentration and quality were then determined using Nanodrop (NANODROP 2000, Thermo SCIENTIFIC). Mix the samples equally according to the concentration of PCR recovered products.
Use TruSeq® DNA PCR Free Sample Preparation Kit library building kit is used to build the library. The constructed library is determined by Qubit and qPCR and then sequenced online using Illumina sequencing platform. The raw reads were deposited into the NCBI Sequence Read Archive (SRA) database (BioProject: PRJNA745259).
Data Analysis
SPSS22 software was used for significant difference analysis of soil physical and chemical characteristics and diversity index, and correlation analysis of soil microbial diversity index, dominant soil microbial groups and physical and chemical properties. Bacterial and fungal communities structure in rhizosphere and non rhizosphere soils were analyzed online using LEfSe (http://huttenhower.sph.harvard.edu/lefse/).
Results and Discussion
Physical and Chemical Characteristics in Soils of Rhizosphere and Non-Rhizosphere
Generally, plants altered soil physical and chemical characteristics by releasing root exudate, and then modify their growth environment [33]. In Robinia pseudoacacia population which located in the Yellow River Delta, the contents of available phosphorus, alkali hydrolyzable nitrogen, organic matter, soluble organic carbon and soluble organic nitrogen in rhizosphere soil were significantly higher than those in non-rhizosphere soil; but no significant difference in the water content, electrical conductivity, pH, available potassium, nitrate nitrogen content between the rhizosphere and non rhizosphere soil [34]. In this study, no significant difference of soil bulk density (SBD) were detected between rhizosphere and non-rhizosphere soil (p>0.05, Table 1), which indicated the uniformity of the soil structure in J. mandshurica plantation. The total nitrogen (TN) in rhizosphere soil was significantly higher than that in non-rhizosphere soil (Table 1, p<0.05), however, lower available nitrogen (AN) content in rhizosphere soil (284.73 mg/kg vs 309.23 mg/kg) seemed to indicate the strong absorption for AN of the roots. The pH value, total carbon (TC), total phosphorus (TP) and available phosphorus (AP) content in rhizosphere soil were 6.15, 2.87%, 0.09% and 12.82 mg/kg, respectively, which were significantly different from those in non rhizosphere soil (p<0.05 or 0.01, Table 1). These results suggested significant differences of physical and chemical characteristics in rhizosphere and non-rhizosphere soil, which might cause by root secretion such as juglone [31, 32] mainly.
Diversity of Bacteria and Fungi in Rhizosphere and Non-Rhizosphere Soils
Bacteria are the largest group of soil microorganisms, the bacterial community abundance and bacterial diversity were affected by habitats in the rhizosphere of Nauclea officinalis in different planting areas [35]. In this study, in total of 55410 and 32791 sequences were obtained from 16S sequencing of bacteria in rhizosphere and non-rhizosphere soil, which were 44445 and 53359 sequences from ITS sequencing of fungi (Table 2). Most of the diversity indexes (Shannon, ACE and Chao1) of bacteria in rhizosphere soil were significantly higher than those in non-rhizosphere soil (p<0.05 or p<0.01, Table 2), which is consistent with the results of poplar plantation [36]. Physiological metabolism of plant roots may be the main reason for the difference between rhizosphere and non rhizosphere bacteria. The enrichment of roots leads to more nutrients near roots. The nutrients in rhizosphere soil are higher than those in non rhizosphere soil, which is conducive to bacterial reproduction, and then increasing soil bacterial communities and the bacterial diversity index [37].
Table 1.
Soil physical and chemical properties in rhizosphere and non rhizosphere.
Table 2.
Soil bacteria and fungi α diversity index in rhizosphere and non rhizosphere.
Fungi are one of the main members involved in the decomposition of soil organic matter and the synthesis of humus, which directly affect soil fertility. And also, the fungi are aerobic microorganisms, which can be used as an indicator of soil aeration [38]. In this study, no significant differences of diversity indexes for fungi were detected between rhizosphere and non-rhizosphere soil (p>0.05, Table 2).
Correlation between Soil Microbial Diversity Index and Physicochemical Characteristics
Nutrient elements and pH value in rhizosphere soil are important factors that affecting soil microorganisms [39]. Person correlation analysis of soil bacterial and fungal diversity index and soil physicochemical characteristics showed that the soil bacterial diversity index in J. mandshurica plantation has significant positive correlation with pH value, total carbon, total nitrogen, total phosphorus and available phosphorus content (p<0.05 or p<0.01; Table 3), but no significant correlation with soil bulk density and available nitrogen content. These results indicated that the significant differences between rhizosphere and non-rhizosphere soils might relate to the pH value, total carbon, total nitrogen, total phosphorus and available phosphorus content. Soil pH affected the rhizosphere microbal community diversity significantly, especially for bacteria [40]. Fierer found that soil pH could explain more than 70% of the variation of bacterial diversity [41].
The four diversity indexes of soil fungi were correlated with soil bulk density negatively and correlated with available phosphorus positively; the ACE and Chao 1 indexes are correlated with pH, TC, TN, AN and TP negatively, and the Shannon and Simpson indexes are correlated with these chemical properties positively (Table 3). However, no significant correlations were detected between the diversity indexes of fungi and the physicochemical properties of soil.
Differences in Composition and Abundance of Microbial Communities in Rhizosphere and Non-Rhizosphere Soil
Seven groups of bacteria with relative abundance larger than 1% in rhizosphere and non-rhizosphere were categorized at the Phylum level (Fig. 1a), among which Actinobacteriota is the absolute dominant groups that accounts for 41.31%-42.57%, and then Proteobacteria accounted for 23.79%-24.94%, Acidobacteriota accounted for 15.00%-16.20%, Chloroflexi accounts for 4.67%-4.71%, Methylomirabilota accounts for 1.90%-2.51%, Gemmatimonadetes accounts for 2.00%2.18%, Myxococcota accounts for 1.55%-1.73% in sequence (Fig. 1a). The bacteria without clear taxonomic status were categorized into others together with the groups of relative abundance less than 1%. The relative abundance of Methylomirabilota in non-rhizosphere soil is higher than that in rhizosphere soil significantly, but no significant difference in the relative abundance of other bacterial groups were detected. The dominant bacterial groups in rhizosphere and non-rhizosphere soil of J. mandshurica plantation are Actinobacteriota, Proteobacteria and Acidobacteriota, whose total relative abundance exceeded 80%. Actinobacteria can promote the decay of animal and plant residues in the soil, and play a certain role in the natural nitrogen cycle [42]. Proteobacteria is the largest phyla in bacteria, which can perform nitrogen fixation and adapt to various complex environmental [43]. Most of Acidobacteriota are acidophile, which is distributed in soil and sediments widely. The the relative abundance of Acidobacteriota increased along with decreasing soil pH. These three groups were also reported as the dominant bacterial groups in lime concretion black soil (Proteobacteria> Actinobacteria>Acidobacteriota) [44], lateritic red soil (Acidobacteriota>Proteobacteria>Actinobacteria) [45] and sandy soil (Proteobacteria>Acidobacteriota> Actinobacteria) [46].
Table 3.
Pearson correlation coefficients between bacteria and fungi α diversity index and soil physical and chemical properties.
Three groups of fungi with relative abundance larger than 1% in rhizosphere and non rhizosphere were categorized at the Phylum level, among which Ascomycota accounts for 78.88%-80.32%, Mortierellomycota 6.26%-7.84%, and Basidiomycota accounts for 2.35%-2.83% (Fig. 1b). Similarly, the fungi without clear taxonomic status were categorized into others together with the groups of relative abundance less than 1% (Fig. 1b). No significant difference between the relative abundance of fungi in rhizosphere and non-rhizosphere soil were detected. These results are consistent with the studies on Lycium ruthenicum in saline-alkali habitats [47] and L. barbarum in different regions of Northwest China [48], of which Ascomycota is also the absolute dominant species. All these results indicated that Ascomycota is the most abundant groups in most soil community, which can effectively decompose plant residues [49].
On the Genus level, in total of 12 Genus of bacteria that relative abundance greater than 1% in rhizosphere and non-rhizosphere were listed in Table 4. Among which, the relative abundance of Bradyrhizobium in rhizosphere soil was significantly lower than that in non-rhizosphere (p<0.05, Table 4), but opposite to the Actinoplanes (p<0.01, Table 4). Bradyrhizobium is one of the beneficial bacteria in the soil, which can provide nutrients for plants through biological nitrogen fixation and facilitate symbiosis with plants. In poplar plantation, the relative abundance of Bradyrhizobium in rhizosphere soil was also lower than that in non-rhizosphere [50].
Fig. 1.
Relative abundance of bacteria a) and fungi b) at phylum in rhizosphere and non rhizosphere in J. mandshurica plantation.
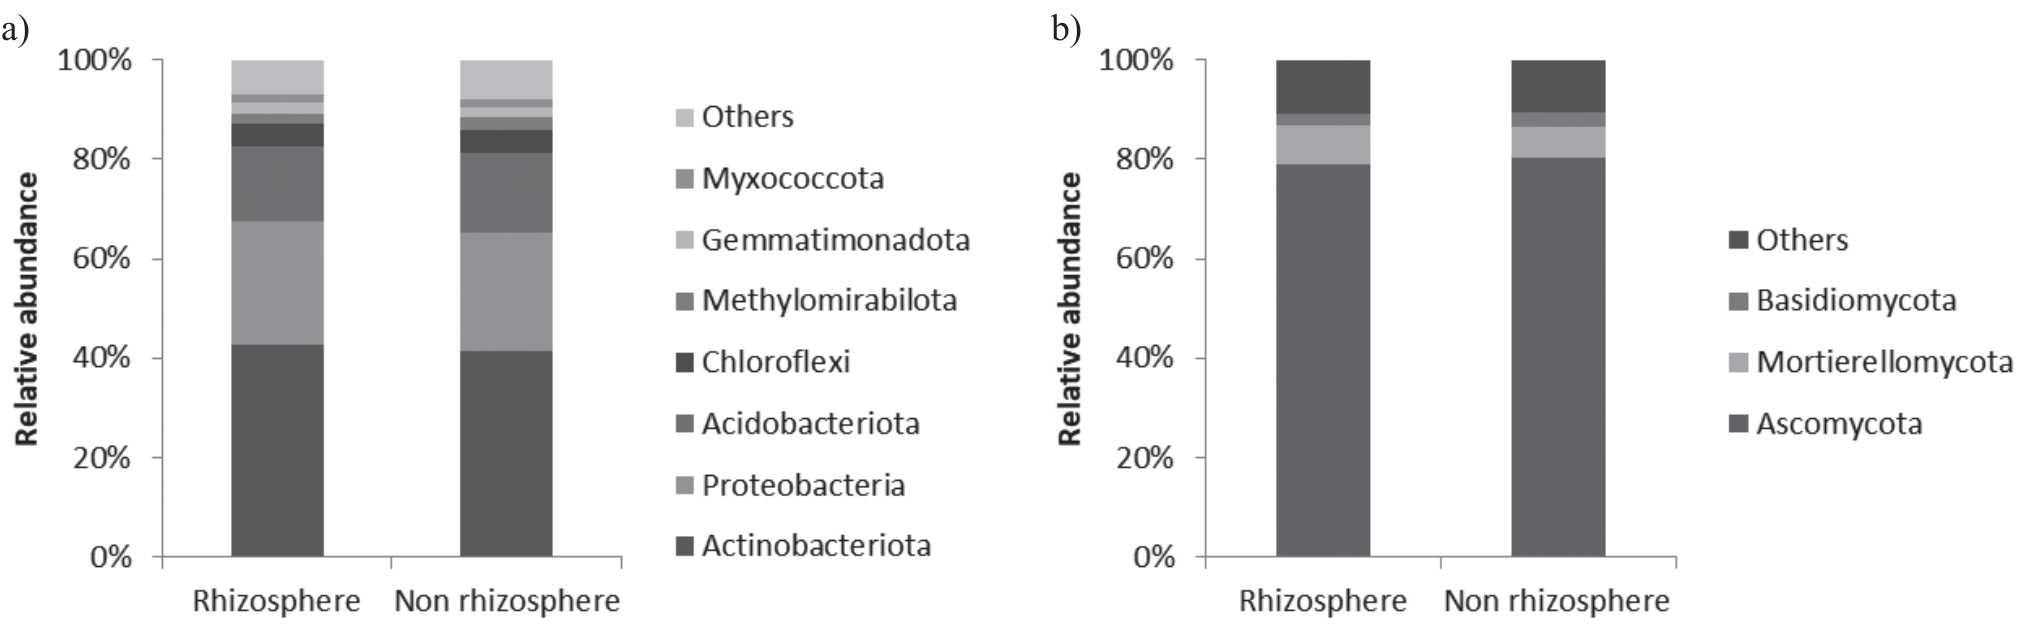
There are 26 fungal genus with relative abundance greater than 1% in the rhizosphere and non-rhizosphere. The top 10 fungal genus with high relative abundance are listed in Table 5, the most abundant genus were Chaetomium, Fusarium, Mortierella, Chaetopyrena, Trichoderma, Cladosporium, Exophiala, Cadophora, Ilyonectria and Nectria in order. Among which, the relative abundance of Cladosporium in rhizosphere soil was significantly higher than that in non rhizosphere soil (p<0.05, Table 5). Cladosporium are pathomycete, which have been reported to cause disease in agriculture and forestry production [51], moreover, they have been reported to degrade cellulose effectively [52].
Correlation between Dominant Microbial Groups and Soil Physicochemical Properties
Pearson correlation between the relative abundance of dominant Phylum categories of microbial groups and soil physical and chemical properties differed greatly, and there are no obvious tendency detected (Table 6). The results revealed less correlation between the relative abundance of dominant microbial groups and soil physicochemical characteristics, except for significant negative correlations between Methylomirabilota (bacteria) and soil pH value (p<0.05, Table 6), or AP (p<0.01, Table 6), and also, significant positive correlations between Basidiomycota (fungi) and AN (p<0.05, Table 6). In rhizosphere soil of Malania oleifera, the relative abundance of Methylomirabilota correlated with AP content negatively (p<0.05) [53], however, no further explaination for this results was reported. In Caragana in semi-arid region in North of China [54], some plant species in water-fluctuation zone in the Three Gorges reservoir area [55] and in alpine meadow in Eastern Qinghai-Tibet Plateau [56], no significant correlation between the relative abundance of Basidiomycota (fungi) and the physical or chemical properties were detected.
Table 4.
Relative abundance of bacterial genus in rhizosphere and non rhizosphere soil.
Table 5.
Relative abundance of fungi genera in rhizosphere and non rhizosphere.
Table 6.
Correlation analysis between dominant microorganism at phylum groups and soil physical and chemical properties.
Biomaker of Rhizosphere and Non-Rhizosphere Soil Microorganisms
In order to find the indicator microorganisms in rhizosphere and non-rhizosphere soil, LEfSe was used to analyze and draw the evolutionary branching map. The evolutionary cladistic diagram of dominant bacteria and fungi is shown in Fig. 2. It is generally believed that the microorganism with LDA (Linear Discriminant Analysis) score greater than or equal to 2 are the biomaker with statistical difference.
Fig. 2.
Bacterial (A) and fungal (B) communities structure in rhizosphere and non rhizosphere soils by LEfSe analysis. Circles from the inner to the outer represent the levels of Kingdom, Phylum, Class, Order, Family and Genus, respectively; and the diameter of the circles is proportional to the relative abundance. The lowercase (sometimes with number) outside of circles replaced the scientific name of corresponding level, which were listed at right. The p_, c_, 0_, f_ and g_ before the scientific name represented Phylum, Class, Order, Family and Genus.
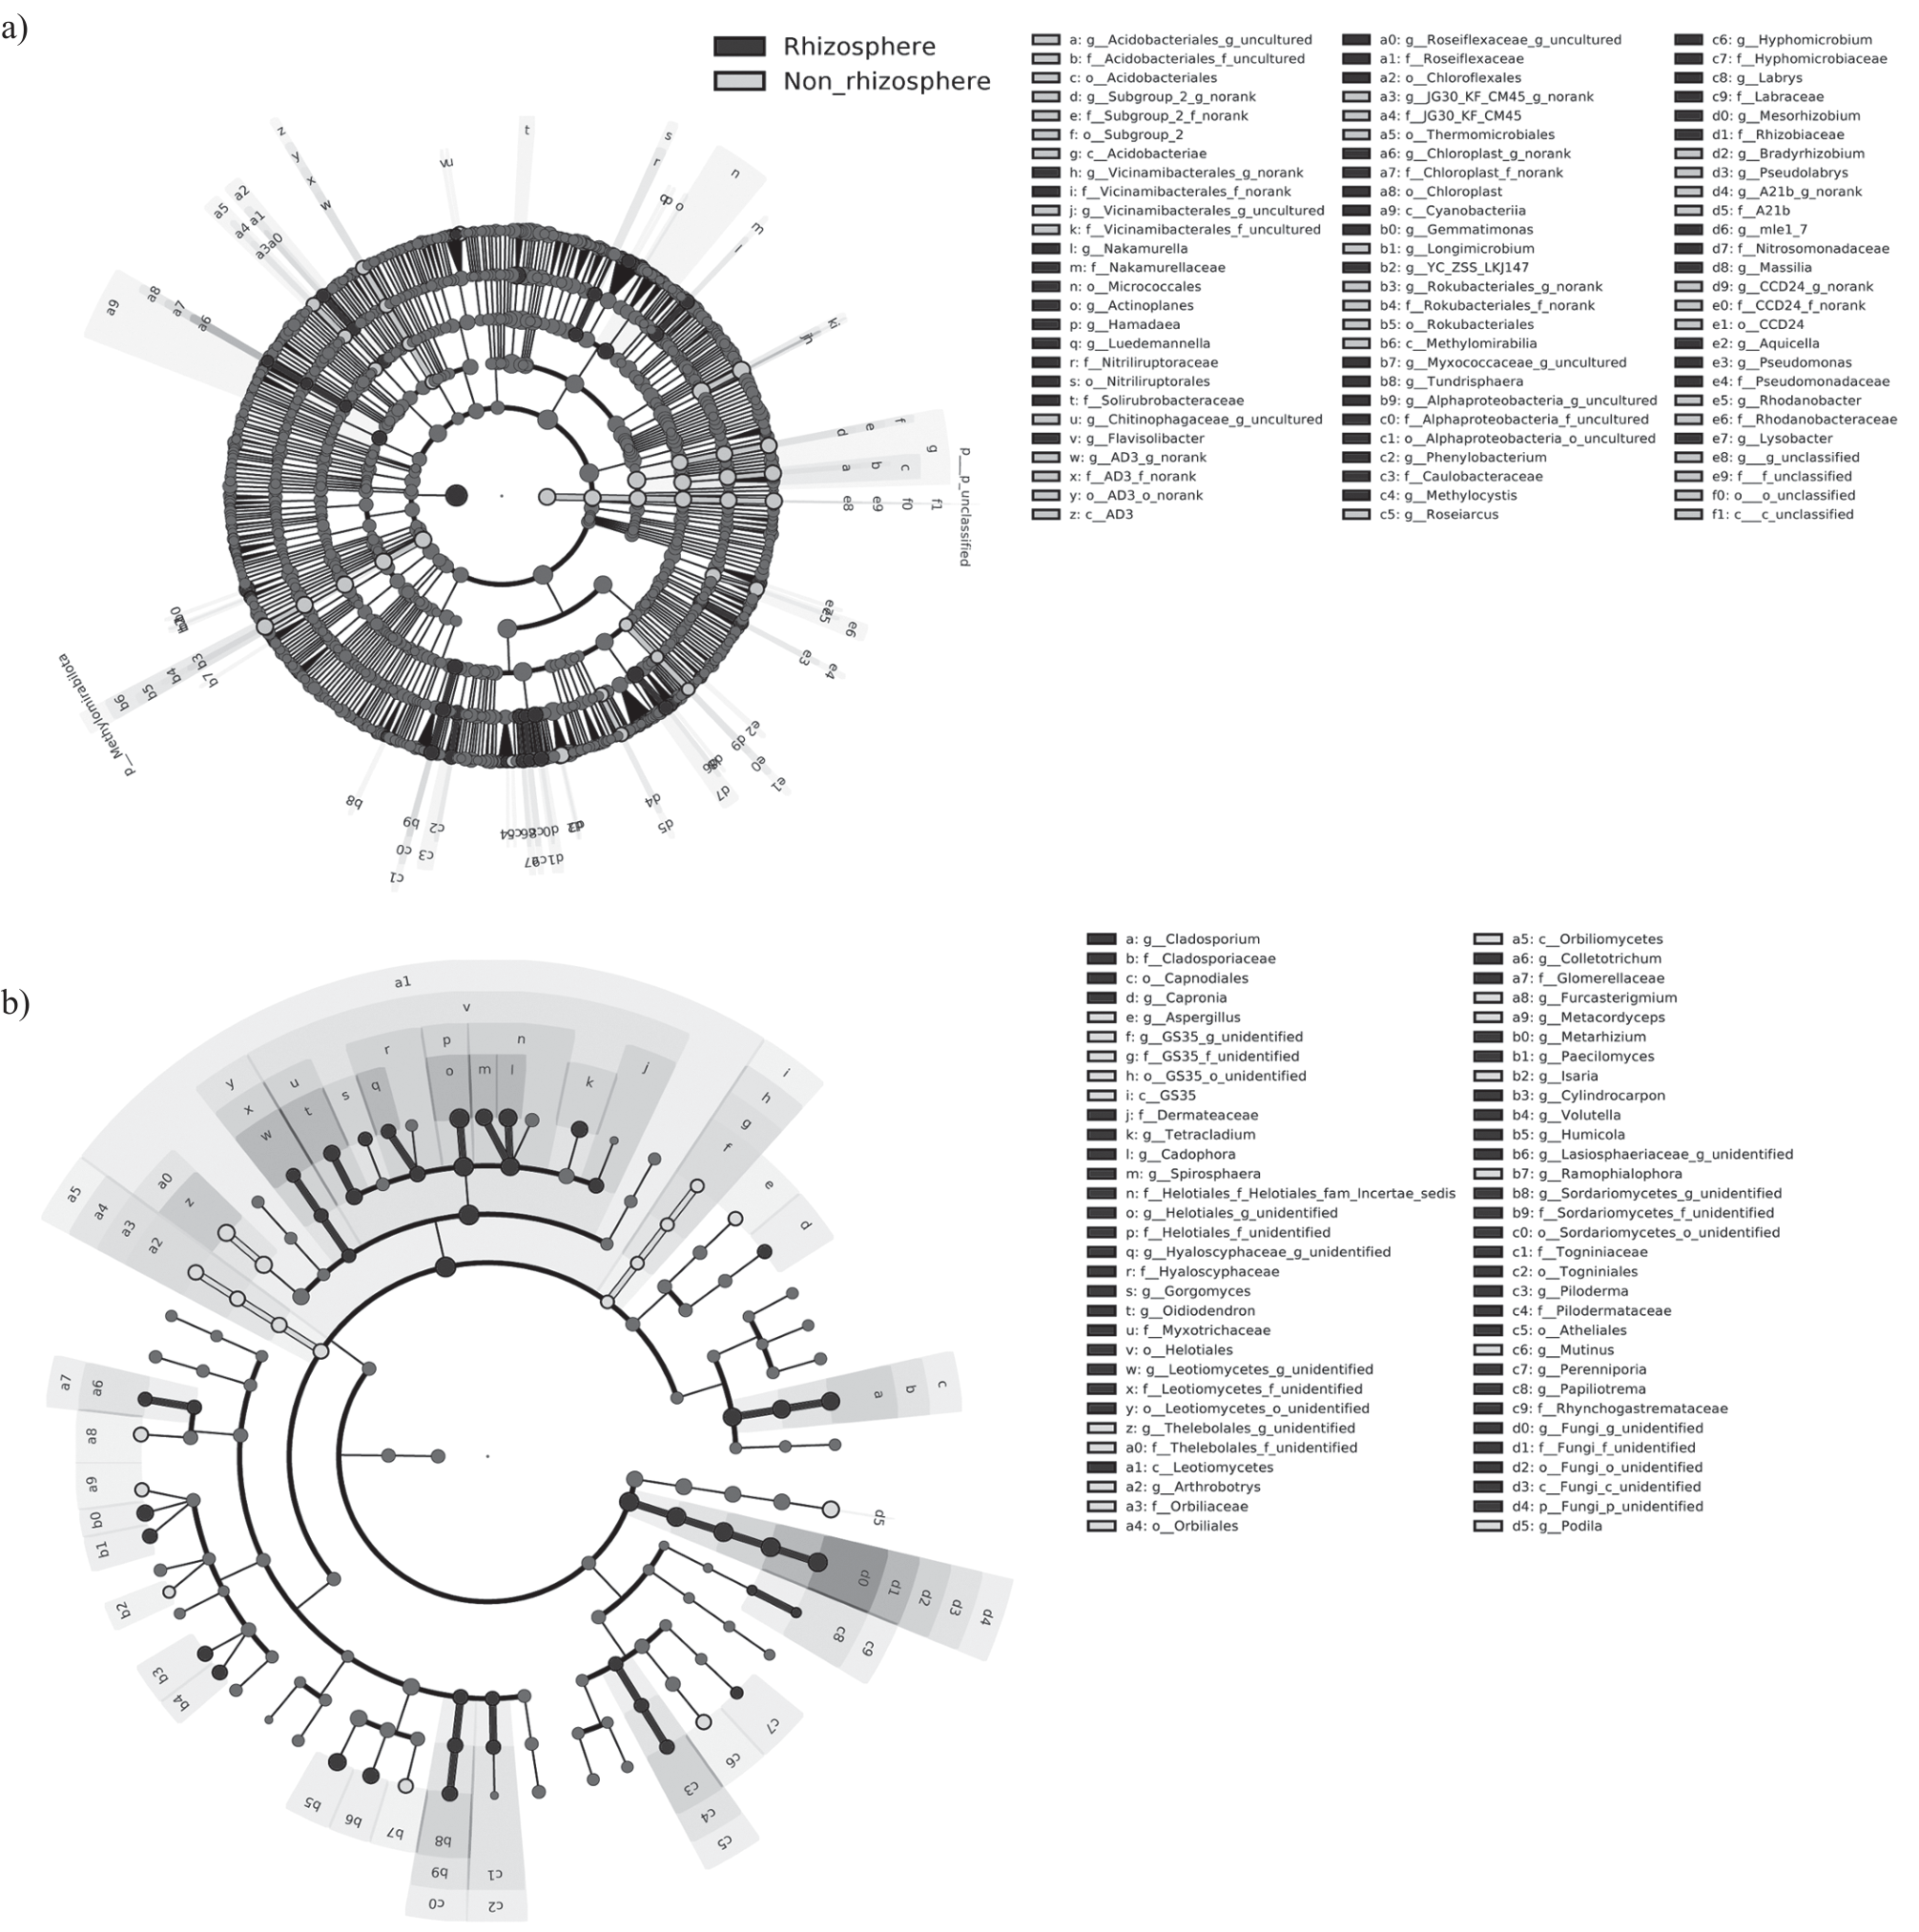
In this study, in total of 82 biomakers of bacteria with LDA score greater than or equal to 2.5 were determined, including 43 in the rhizosphere soil and 39 in the non-rhizosphere soil. The dominant bacteria categories in the rhizosphere and non-rhizosphere differed greatly, but no significant difference in the number of biomakers. The dominant biomakers in the rhizosphere soil mainly include Family Nakamurellaceae (of which Nakamurella is the most abundant genus), Order Micrococcales, Genus Actinoplanes and Hamadaea, etc; and the dominant biomaker in non rhizosphere soil mainly include Class Acidobacteriales, Order Thermomicrobiales, Genus Longimimicrobium, Class Metallomirabilia, etc (Fig. 2a).
The number of fungi biomakers in rhizosphere and non rhizosphere soil varies greatly, in total 62 biomakers were determined, of which 45 were detected in rhizosphere soil and 17 were detected in non rhizosphere soil (Fig. 2b). The dominant fungi biomakers in rhizosphere soil mainly include Order Helotiales (of which most genus are high abundant), Order Leotiomycetes (almost all of species were determined as genus Leotiomycetes), Order Capnodiales (almost all of species were determined as genus Cladosporium), etc. The dominant fungi biomaker in non rhizosphere soil mainly include genus Podila, order Orbiliales (almost all of species were determined as genus Arthrobotrys), etc (Fig. 2b).
These results implied the large differences of indicator microorganisms in rhizosphere and non-rhizosphere soil, which might cause by the selective recruitment of microorganisms from the non-rhizosphere soil, and then drive the assembly of rhizosphere microbial communities [57]. Generally, plants could alter the relative abundance or diversity of some bacteria and form a beneficial microbial community structure by roots metabolic activity [58].
Conclusions
In this study, the physical and chemical characteristics (total carbon, total nitrogen, pH value, total phosphorus and available phosphorus) of rhizosphere and non-rhizosphere soils in J. mandshurica plantation differed significantly. Of which, soil pH value and available phosphorus were the main factors affecting soil bacterial community structure in J. mandshurica plantation; and the soil available nitrogen is the main factor affecting soil fungal community structure. Significant difference of the bacterial diversity indexes and bacteria categories between rhizosphere and non-rhizosphere soils were detected. And for fungi, significant difference of the number and the categories of fungal biomaker between rhizosphere and non-rhizosphere soils were detected, however, there was no significant difference of the fungal diversity indexes between rhizosphere and non-rhizosphere soils. However, why and how did the physical or chemical characteristics affect the soil microbial community? The issues should be resolved by studying the categories and metabolism of root exudates, and by studying the categories and functions of the indicator microorganisms identified. Moreover, it is also necessary to study the changes of microbial communities structure by altering soil physical and chemical characteristics artificially (e.g. fertilization).

