

Introduction
CO2, a requisite for the global carbon cycle, undergoes a reduction reaction during photosynthetic carbon metabolism to provide necessary food, energy [1], and organic building blocks for almost all living beings. Thus, CO2 becomes a predominant environmental signal and living factor for physiological responses in many photosynthetic organisms [2]. It is one of the crucial elements required for the sustainable production of fuels [3]. However, due to the industrial revolution, anthropogenic activities like massive combustion and consumption of nonrenewable fuel have significantly increased CO2 levels (approx. 65%) in the atmosphere, accompanied by a significant rise of heavy metal pollutants [4]. Monitoring and mitigating high CO2 and heavy metal pollution in the air are essential for safeguarding environmental quality. Plants Nerium oleander and Picea orientalis L. have been identified as the most suitable biomonitors for cadmium and chromium heavy metals, respectively [5, 6]. According to the NOAA Earth System Research Laboratory (2022), the atmospheric CO2 threshold was breached from 280 ppm to 417.06 ppm between the 18th century and the 20th century, respectively. Despite the above uses, increased CO2 levels and other greenhouse gases trap heat from the atmospheric surface and cause steady planet warming. All through the pre-industrial times, the global mean temperatures elevated by 2-3ºC due to global warming [7], a critical circumstance in the last two decades. On the other hand, according to the Indian Institute of Tropical Meteorology Metrics, the Tropical and Western Indian Oceans experienced a rapid increase in ocean surface warming at a rate of 0.15 degrees Celsius per decade and a four-fold rise in heat waves, respectively [8].
Elevated temperatures and intensive heat waves are the major threats to the global food supply [9]. One of the instances is the U.S. heat waves in 1980-1988, which culminated in billion-dollar damage to agricultural production [10]. During plant growth, at high temperatures, the ability of Rubisco O2 fixation increases rather than CO2, instituting unproductive pathways that hinder crop yield [11]. Hence, any switch in the optimum CO2 concentration and temperature in the atmosphere will profoundly impact plants’ photosynthetic growth and carbon metabolism [12].
To overcome these high atmospheric temperatures, there is a need to develop direct CO2-capturing negative carbon emission technologies to mitigate CO2 from the atmosphere. Bioenergy with carbon capture and storage (BECCS) is considered the most effective negative CO2 emission technology, having high-profile potential in removing global carbon dioxide and bioenergy benefits [13]. One of the promising BECCS is the microalgal-based biological CO2 mitigation [14]. Here, the CO2 from the atmosphere is sequestered indirectly by algal photosynthesis, which is utilized further for energy-generating products like fuels and food. This pathway of CO2 mitigation can limit climate warming to 1.5 or 2ºC [15].
Photosynthetic unicellular green algae are eukaryotic organisms that play an important role in the land and aquatic ecosystem as excellent biosensors for environmental monitoring. They provide nearly half the earth’s oxygen by sequestering CO2 into the biological systems through CCM. Hence, culturing the algae that possess CCM was advised to be a sustainable green technology with beneficial CO2 sequestration [1]. Algae have been recognized as super plants of the future because they can be grown and harvested year-round and are also feasible for renewable biofuel production [16]. There are approximately 100,000 microalgae species, each with its own distinct set of properties. In addition to mitigating CO2 emissions, they can reduce excess nutrients and treat heavy metal-contaminated effluents by breaking down and imbibing the contaminants through processes like biosorption, bioaccumulation, and biotransformation [17]. This diversity allows microalgae to flourish in almost every environment on Earth [18]. The unicellular green algae Chlamydomonas reinharditii is an important model organism to study photosynthesis [3] because its photosynthetic system, light physiology, and carbon assimilation process are similar to higher plants [19]. Ecologically, the genus Chlamydomonas is found worldwide, with species of this algae thriving in a wide variety of habitats: They can be collected from environments such as humid areas, varying temperatures, saline conditions, and damp soils, as well as fresh, marine, and sewage waters. Additionally, some of these species are known for their tolerance to pollution [20]. In addition, these cells can also be cultured under controlled conditions, and changes in environmental conditions can be applied homogeneously [21]. The availability of whole genome sequence and mutant libraries of Chlamydomonas helps understand the changes in protein abundance under different stresses [22]. In the scenario of peak carbon dioxide and global warming conditions, microalgae are recognized as effective agents for mitigating CO2 emissions. Henceforth, there is a need for study to understand the photo-physiology, CCM-related gene expression, and CO2-mitigating efficiency of microalgae that possess well-organized CCM concerning mechanisms under the increased temperatures.
How Does the Approach of Algal CCM Assist in Curbing CO2 Pollution and Temperature?
Under the circumstances of high carbon dioxide levels and subsequent global warming, the Intergovernmental Panel on Climate Change (IPCC) disclosed two pathways to reduce the rate of high temperatures by about 1.5-2.0ºC per year. These pathways include reducing and removing CO2. a. Reducing CO2 involves limiting our reliance on
fossil fuels. b. Removing CO2 involves methods that actively uptake
atmospheric CO2.
The solution for carbon removal starts with photosynthetic organisms because they absorb atmospheric carbon dioxide through photosynthesis and convert it into organic carbon. Microalgae are considered highly efficient photosynthetic organisms because of their capacity to consume 2-10 times more CO2 and produce 15-300 times more biomass efficiently than land-based plants [1]. This is because of the peculiar carbon fixation mechanism called CCM [23]. Microalgae with biophysical pyrenoid-based CCM plays a crucial role in assimilating ca. 40%-60% of global carbon dioxide each year [24]. This large amount of CO2 fixation accounts for a large portion of global primary productivity [25]. CCM is an evolutionary adaptation acquired by microalgae and cyanobacteria to counter the negatives of RuBisco and the aquatic environment [26]. In aquatic environments, microalgae face a 10,000- fold slower diffusion rate of CO2 compared to that of the terrestrial atmosphere [27, 28]. To get over this limited CO2 environment, microalgae like Chlamydomonas and other aquatic photosynthetic plants actively capture the high amount of CO2 in the form of inorganic carbon (Ci; CO2 and HCO3-) into the cell through this unique carbon capture system and increase the level of CO2 at the site of RuBisco [27].
As CCM-adapted microalgae are highly efficient in CO2 fixation and biomass productivity, understanding how atmospheric CO2 and temperature levels influence the mechanism and regulation of microalgal CCM at the cellular and molecular level is very predominant [26]. In addition, analyzing the adaptive response and recovery capacity of microalgae and plants to high temperatures probably extends our perception of thermostability in all plants and algae [29].
In this scenario, CCM gains significance in studying the obtaining efficiency of CO2 in the cells under increased temperatures. Understanding the global climate change factors like CO2 and temperature conjointly might give a broad scope of how these changes impact plant growth and metabolic networks.
Why Is an Optimum Temperature Considered to Be an Essential Factor in Living?
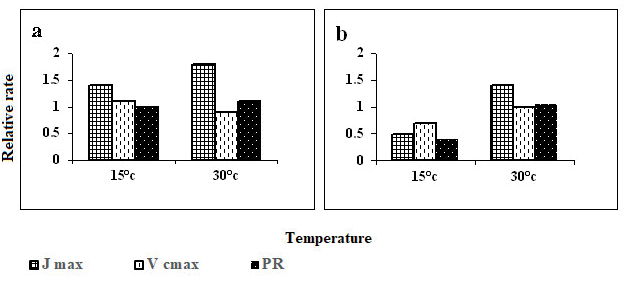
The majority of physiological functions and enzymatic activities in living organisms highly depend on temperature [30]. The changes in temperatures have an impact on cellular processes at different stages [31]. Photosynthesis was one of the cellular processes where the rate of RuBP carboxylation (Vcmax), electron transport/RuBP regeneration (J max), and the ratio between Vcmax & J max altered according to the growth temperatures [32] (Fig. 1). Similarly, at high temperatures in the diatom, Phaeodactylum tricornutum uptake of Ci and concentration of Ci at the site of RuBisco and the kinetics of CCM components change [33]. However, these responses are specific to particular species at their particular growth temperature. Plant cells thrive in the above-optimum range temperatures by adapting some acclimatory mechanisms. Chlamydomonas cells, as an acclimation process, activate heat shock chaperons, proteins (HSP & HSF), upregulate photosynthesis and CCM [34], and thermotaxis genes [35]. The temperature sensitivity of CCM components varies according to imbalanced Ci fluxes resulting from temperature fluctuations. Therefore, microalgae maintain balanced Ci levels by synchronizing their CCM components to temperature variations, supporting highly efficient photosynthesis [33].
How Do Chlamydomonas Cells Sense Temperature?
Plants and microalgae sense changes in surrounding temperatures via a network of molecular detectors located in different cell compartments, i.e., plasma membrane (PM) sensing via the influx of calcium (Ca+2), unfolded proteins (UP) in the endoplasmic reticulum, cytoplasm, and chloroplast, and increased membrane fluidity [36, 37]. This heat stress signaling process was activated primarily when the photosynthetic apparatus of the chloroplast was subjected to damage by thermal stress [38].
A combination of electrophysiology, reporter gene assays, and biochemical measurements revealed that Ca+2 channels sense a mild increase in temperature at the PM. These channels open due to increased membrane fluidity and activate the influx of Ca+2 ions [37, 39, 40].
Fig. 1.
Bar chart representing the variations in photosynthetic rate (PR), RUBP regeneration (J max), RUBP carboxylation (V max) at 350 μmol mol⁻ ¹ CO2, 15ºC (a) and 30ºC (b) in Quercus myrsinaefolia (redrawn from Hikosaka et al., 2006).
Studies with Arabidopsis report that the PM cyclic nucleotide-gated channels (CNGC) are well-known transport channels. These channels are activated when the membrane fluidity/cAMP levels increase due to heat stress-activated adenylyl cyclase leading to Ca+2 influx. Knockdown of the cngc6 gene in Arabidopsis shows no active calcium influx followed by reduced thermotolerance [37]. Thus, the accumulation of intracellular Ca+2 in the cell during heat stress ensures that the calcium-reliance signaling system plays a signature task in response to thermal stimuli [41]. Recently, a putative Ca+2 voltage-gated channel gene (CAV4) was identified in Chlamydomonas, which was supposed to be activated at high temperatures of 35ºC [34].
Another temperature sensor in Chlamydomonas is a cation-selective sensory ion channel called transient receptor potential channel TRP1. Upon heat stress, the opening of the TRP1 channel was mediated by increased levels of phosphatidylinositol-4,5-bisphosphate (PIP2) in the cell. These TRP channels were also known to regulate cellular Ca+2 uptake in Ulva compressa and Ectocarpus siliculosus [42]. However, Ca+2 influx through this TRP1 channel in Chlamydomonas was understudied.
Interestingly, CCM gene regulation by Ca+2-mediated retrograde signaling from chloroplast to nucleus was discovered recently [1, 2]. Since Ca+2 is involved in sensing both CO2 and temperatures, the functioning of Ca+2-mediated channels and their regulation during fluctuating temperatures and CO2 levels need to be examined.
Results and Discussion
Temperature-Induced Primary Protective Mechanism Adopted by Chlamydomonas
Chlamydomonas and other photoautotrophic organisms in the wild are exposed to environmental stress, like fluctuations in the surrounding temperature. Plants recognize temperatures exceeding the optimum range as heat stress (HS) [43]. This kind of exposure to high temperatures disturbs many cellular processes, such as disturbances in assembling protein complexes, protein folding, cell membrane fluidity, cellular metabolism, enzymatic reactions, cell division, DNA replication, and repair. These disturbances trigger the production of molecular chaperones called heat shock proteins (HSP) [37, 44, 45].
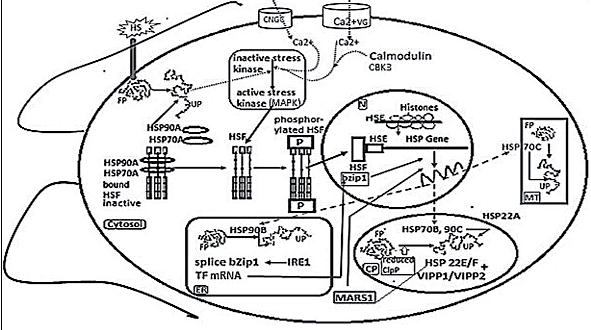
HS response was regulated at the transcriptional level by transcription factors called heat shock factors (HSFs). In plants, at optimum temperatures, heat shock protein (HSP) gene transcription by heat shock transcription factors was kept inactivated by bound HSP70-HSP90 chaperones in the cytosol and enwrapped HSP genes by histone proteins in the nucleus. Upon mild warming (priming), thermo-sensors signal to activate the transcription of HSP genes by dissociating the inhibitory HSP70-HSP90 chaperones from HSF. In Chlamydomonas, of the two HSFs, HSF1 & HSF2, HSF1 is a canonical HSF [37, 39] that is structurally trimeric and undergoes phosphorylation at the time of heat stress, binds to the promoter region of HSP genes, and initiates transcription leading to the proliferation of HSP transcripts [37] (Fig. 2). The most abundant HS chaperones expressed were cytosolic chaperones – HSP90A, HSP22A, and HSP70A; Plastid chaperones – HSP70B, HSP90C; and mitochondrial chaperones HSP70C and ER luminal – HSP90B [37].
During heat stress, increased levels of Ca+2 and UP in the cell activate the stress kinases. These active stress kinases trigger the activation of HSF, which in turn promotes HSP gene expression in the nucleus [37, 46, 47]. In Chlamydomonas, unfolded protein accumulation along with Ca+2 and calmodulin-binding kinase (CBK3) activate inactive stress kinase mitogen-activated protein kinase (MAPK), which leads to the activation of HSF [48, 49] (Fig. 2). This was supported by the work done with Chlamydomonas, where the cells treated with BAPTA, a Ca+2 chelator, exhibited a low and delayed expression of the HSP gene and decreased thermotolerance under heat stress [37]. Even though Ca+2 chelators inhibit Ca+2 influx from the exterior, the heat stress response was induced in the cell by the intracellular Ca+2/calmodulin-dependent HS signaling mechanism [50]. Hence, both extra and intracellular calcium levels influence heat sensing.
Chloroplast heat shock chaperones/HSPs play an essential role in obtaining thermotolerance. They protect and stabilize the photosynthetic mechanism and the apparatus under increased temperatures [38]. In chloroplasts, the heat stress state signal is coordinated at HSF1, where heat stress is sensed and transferred to the nucleus to generate HSF and HSPs. During heat stress, chloroplast protein (Clp) protease degradation in chloroplasts led to misfolded proteins. This downside action was detected and sequestered by small HSPs (HSP22E/F) and vesicle-inducing plastid proteins (VIPP1/VIPP2) located in the chloroplast membrane. This process triggered a retrograde signal to the nucleus through cytosolic mutant affecting retrograde signaling 1 (MARS1) kinase, leading to the upregulation of the HSPs [48] (Fig. 2). This finding is supported by the work on the HSF1-RNA i strain, a mutant lacking the HSF1 gene, which completely lacks transcripts of the chloroplast chaperone HSP90C [40]. Chloroplast stromal HSP70B in C. reinhardtii and Dunaliella was reportedly involved in the molecular protection and repair of photosystem II (PSII) [36]. Small heat shock proteins Hsp22E/F are noticed upon interacting with RuBisco activase, RCA1, under heat stress for optimal activity [47]. Another retrograde signaling system that initiates during HS is in the ER. In the ER, unfolded protein accumulation at the time of HS leads to the activation of inositol-requiring enzyme I (IRE1) RNase activity. This active IRE1 splices the mRNA of the basic leucine zipper 1 (bZIP1) transcription factor. bZIP1 produced from the spliced mRNA acts as a retrograde signal in the nucleus, upregulating the HSPs [48] (Fig. 2).
Influence of Temperature on Photosynthetic Light Machinery and Their Reciprocal Acclimatory Reactions
Photosynthesis is one of the most important physiochemical processes of both higher plants and algae. These autotrophic organisms carry photosynthetic apparatus that exhibits a characteristic feature of sensing different environmental changes such as temperature, CO2 levels, nutrient availability, light quality, and quantity by rapid adjustment or acclimation [51]. Thus, the enzymes and the genes involved in the functioning of the photosynthetic apparatus and their mechanisms are highly susceptible to different stresses [36]. Although photosynthesis is purely a light-dependent process, it requires sufficient temperature because all a cell’s metabolic and enzymatic activities depend on the optimum temperature [52]. Since the greenhouse effect, plants face additional temperatures up to 45ºC; these high temperatures cause a large depletion in plant yield [53]. The growth of photosynthetic organisms may increase with increased temperatures to a certain degree; later on, the growth decreases when the temperature surpasses a certain heat threshold. This decrease in growth is due to the decreasing photosynthetic efficiency. Efficient photosynthesis occurs only when electron transport and thylakoid membrane complexes coordinate collectively during the light reaction and carbon fixation cycle, respectively [31]. Disturbance in the light reactions indirectly affects the carbon fixation cycle by the inefficient production of ATP and NADPH during abiotic stress conditions. Therefore, the photosynthetic apparatus (PA) within the chloroplast is considered the primary structure prone to thermal stress damage [38]. This damage leads to improper carbon fixation, ion leakage, increased thylakoid membrane fluidity followed by the unordered arrangement of PS-II, PS-І, the cyt b6f complex, and ATP synthase, and finally, disturbances in energy distribution between photosystems, which eventually reduces the rate of electron transport followed by decreased yield [54].
Photosystems are the major target of high temperatures. Of the two photosystems (PS-II/PS- І), the reaction center (RC) PS-II is considered the most thermosensitive complex and the foremost target of heat inactivation of photosynthetic light reactions [55]. The imbalance between light absorption and electron transport during high temperatures leads to the over-excitation of PS-II RC. In an over-excited state, chlorophylls’ high energy reacts with molecular oxygen to release reactive oxygen species (ROS). These products damage the PS-II protein subunit D1, leading to photoinhibition [31] along with the respective detachment of Mg²⁺ ions, extrinsic proteins of the oxygen-evolving complex/water oxidizing complex (OEC/WOC) [55]. In addition, electron transfer kinetics between QA & QB on the PS-II donor and acceptor sides play an essential role in PS-II photoprotection and the electron transport chain [56]. Though PS-II reaction center protein subunit D1 is the main target of light-induced damage, changes in amino acids of D1 protein and regulation of D1 protein synthesis during elevated temperatures were reported [36]. Work with spinach thylakoids under heat stress reports that the loss of PS-II activity occurs due to the cleavage of D1/PsbA protein and the release of extrinsic proteins of PS-II. PsbO/OEE1 is one such extrinsic protein of PS-II that aids in stabilizing the manganese cluster, whose loss results in destabilization and degradation of the entire PS-II complex. Tolerance of spinach PS-II to high temperatures was achieved by replacing mesophilic PsbO with a PsbO of thermophilic cyanobacteria [3].
Although high temperatures distract the photosynthetic machinery of photosynthetic organisms acclimated to such conditions, they express enhanced thermal stability [57]. This stability phenomenon has been observed in several species of higher plants and cyanobacteria. Recent studies report upregulating about 200 chloroplast-allied genes at high temperatures in plants [58]. Some genes that were upregulated during elevated temperatures in Chlamydomonas are listed in Table 1. Temperature-acclimated cells display a highly thermostable PS-II reaction center because of the high stability of oxygen-evolving machinery [59]. This stable activity of WOC/OEC is due to its extrinsic proteins PsbO, PsbP, and PsbQ; these proteins act as a shield over the Mn cluster of OEC and improve the O2-evolving efficiency of PSII. Along with these extrinsic proteins, OEC is supported by intrinsic luminal heterodimer proteins D1 and D2 and chlorophyll-binding proteins CP43 and CP47. Also, seven amino acids, six from D1 and one from CP43, coordinate the Mn cluster with PS-II [60, 61]. Even the lack of a single protein causes remarkable conformational changes. Cyanobacterium synechococcus sp. mutant with a defective PsbU gene could not increase the thermal stability of oxygen-evolving machinery and cellular thermotolerance upon acclimation to high temperatures. This inactivation of oxygen-evolving machinery was stabilized by replacing cytochrome (Cyt) C550 and PsbU proteins of PS-II [62, 63].
Table 1.
List of candidate genes, their related information & temperature regulation.
The robust nature of the thylakoid membrane protects photosynthetic apparatus from the damage caused by abiotic stress. This is due to peculiar actions like alteration of the electron transport pathway, light-harvesting complex II (LHC-II) rearrangement, and PS-II/PS-І stoichiometry [55]. Though photosynthetic algae and plants regulate their photosynthetic antennae according to light, temperature shifts often alter their light-harvesting antennae and LHC expression [64]. The state transition is a major mechanistic response that alters during abiotic stress. The state transition is a reversible excitation balancing mechanism that operates within minutes to balance the electron transport between PS-І and P [13]. Recent studies with Chlamydomonas revealed that the mechanism of light-induced state transitions varies from temperature-prompted state transitions. Under elevated temperatures, the decreased carbon fixation process at the PS-I acceptor side causes over-excitation of PS-II, reducing the plastoquinone (PQ) pool. This PQ pool reduction phosphorylates LHC-II by activating STT7/STN7 kinase. In the dark at high temperatures, phosphorylated-LHC-II detaches from PS-II and does not bind to any photosystems, but on recovery, a fraction of P-LHC-II binds to PS-І. In the light-induced state transition, the phosphorylated LHC-II of PS-II immediately detaches and binds to PS-I. Other aggregates, such as PS-II-LHC-II-PS-I and PS-I-Cytb6f, were also observed during light-induced state transition. P-LHC-II allocation during state transition might prevent photo-oxidative damage from combined high light and temperature intensities [55]. Recent reports with Chlamydomonas disclosed that high temperature (40ºC) and light accelerate the formation of the PS-I cytochrome b6f complex and elevate cyclic electron flow (CEF) activity. This CEF maintains the equilibrium of ATP and NADPH, develops a proton motive force, and safeguards both PS-I and PS-II from photo-oxidative damage [34].
Temperature Versus Carbon Dioxide Fixation and Acclimatory Responses
The reduced rate of photosynthesis during heat stress is more likely due to reduced capacities of downstream reactions rather than damage to PS-II. One of the downstream reactions affected was the Calvin cycle/ photosynthetic carbon reduction cycle. In the aquatic environment, increasing temperatures cause the upper mixed layer of water to become shallower. This results in an increased mean flux of PAR (photosynthetically active radiation) and UV-B, decreasing the supply of nutrients, including inorganic carbon [26]. A sufficient concentration of carbon source is necessary for a successful Calvin cycle. To avoid CO2 deficiency, aquatic plants and microalgae actively uptake Ci (CO2 and HCO3-) and transport them to the pyrenoid, which is rich with the RuBisco enzyme, through CCM. This active intake and transport is accelerated by the action of Ci transporters and carbonic anhydrases (CA) [23, 28, 65]. Hence, photosynthetic organisms are scheduled to have adequate CCM activity to a greater extent for effective photosynthesis [65]. Increased temperatures boost the CO2 unavailability in the local environment and subsequently decrease the RuBisco affinity to CO2, resulting in reduced photosynthetic efficiency [66]. Due to the Ci fluctuations caused by high temperatures, microalgae have to regulate the CCM accordingly to maintain balanced Ci levels and photosynthetic efficiency.
The RuBisco/RuBisco activase is a highly thermolabile enzyme complex, and its affinity for CO2 decreases at high temperatures [21]. Work with spinach reports that an 80% reduction in CO2 fixation rate under heat stress occurs due to the thermolabile nature of RuBisco [37]. However, a recent report discloses that RCA1 protein interacts with Hsp22E/F to support optimal RuBisco activity during high temperatures [47]. Because RuBisco is heat sensitive, heat shock proteins detect the unfolded proteins and fold them during stress as a primary protective mechanism to safeguard the activity of RuBisco and the subsequent CO2 fixation cycle.
Carbonic anhydrases are crucial metalloenzymes that catalyze the interconversion of CO2/HCO3-. These enzymes aid in the rapid supply of carbon dioxide and bicarbonate for various metabolic pathways such as photosynthesis; they are also involved in ion exchange, pH regulation, and Ci diffusion (carboxylation) [67]. During the daytime, due to high irradiance and high temperatures above 45ºC, plants face dual stress, leading to the fall of pH up to 5.5 in the thylakoid lumen, inhibiting PS-II activity [68]. In Chlamydomonas, maintenance of a functional CCM depends on the pH gradient that occurs during the light reactions. Thus, the formed pH gradient results in the basic stroma with pH 7.5-8.0, while the thylakoid lumen becomes acidic with pH 5.8-6.5. This acid pH range in the thylakoid lumen favors the CA to convert HCO3- (Ci) to CO2 [67]. Hence, the occurrence of low pH in the thylakoid lumen during high temperatures of up to 40ºC probably supports CCM by increasing the CA activity for sustainable and efficient photosynthesis. Further research is needed to understand how various environmental stresses, such as CO2, temperature, light, pH, etc., regulate the CAs.
As discussed earlier, light reaction and the processes of CO2 fixation work together in an interconnected manner. PS-II oxygen evolutionary machinery exhibited a close association with carbonic anhydrase activity and bicarbonate ions. HCO3- is said to be one of the ionic cofactors involved in splitting water molecules. This anion is produced by PS-II from H2O and CO2, confirming that PS-II has the CA activity. Which component of PS-II involved in CA activity was analyzed by immunoblotting assay? This assay revealed that the CA gene sequence that migrated on SDS PAGE was positioned equally to the OEC33, also known as the 33 KDa extrinsic protein/manganese-stabilizing protein. So, from the above work, it can be concluded that the source of PS-II CA activity would be the OEC33. This is evidenced by analyzing the CA activity of purified OEC33 protein in Escherichia coli cells. These cells lack CA activity in the presence of Zn2+ while exhibiting CA activity in the presence of Mn2+. Since the manganese ion is an active site of OEC, PS II-OEC is proven to possess CA activity. The CA activity that was noticed here could be the thylakoid lumen protein CAH3 because this CAH3 protein is said to be associated with the donor side of the PSII complex, and it is essential for the stability of the Mn cluster and WOC [1]. The bicarbonate ion released by the enzymatic action of CA activity of CAH3 protein accelerates the formation of Mn clusters to attain stability. OEC33/OEC is highly heat stable; it can still reengineer the oxygen evolution after heating to 50ºC for 15 min [69]. The major action noticed was that even at these high temperatures, CA activity was not less, yet it became higher after heating than before [70]. This increased CA at high temperatures might be due to decreased pH levels in the thylakoid lumen. The acidic range of 4.5-5.7 supports the oxygen-evolving activity [71]. Although pH levels decrease at high temperatures, the oxygen-evolving activity remains active in acidic conditions, as noted above. This consistent activity supports the stable CA activity of PS-II. As evidence for the above statement, system-wide analysis of mixotrophically grown Chlamydomonas cells during acute temperatures up to 40ºC exhibits that most of the transcripts of CCM were upregulated as a consequence of maintaining the sufficient amount of CO2 concentration at the site of RuBisco in the pyrenoid [34]. Henceforth, at high temperatures (38 and 40ºC), the acclimatory responses, such as stabilized PS II-OEC activity and increased CA activity in the thylakoid lumen, manage stable CCM and increase the CO2 levels at RuBisco to maximize the photosynthetic efficiency because the availability of CO2 decreases with increased temperatures. In Chlorella species, the DIC-dependent photosynthetic O2 evolution rate (i.e., the capacity of DIC utilization) and the value of Pmax were greatly enhanced in the M4 (thermo-tolerant) mutant grown under 40ºC, 200 μmol/m2/s⁻¹, and 6% CO2 conditions compared to the wild type (exhibiting decreased PS-II activity). This enhanced high thermotolerant mechanism is probably due to the gene mutations in their related components, such as genes involved in enhanced Pmax value (enlarged PS-II number) and CO2 fixation process (the function of CO2 utilization and Calvin cycle) under elevated temperatures [72].
This review highlights the various acclimatory responses that play an important role at each stage of the photosynthetic carbon fixation process, enabling stable photosynthesis during high temperatures. More work is needed to understand how these processes are interrelated and to identify the genes involved in acclimatory responses to abiotic stresses such as light, temperature, and CO2 levels.
Conclusions
To minimize our carbon footprint, the efforts are focused on MBECCS because of its high CCM efficiency and year-round cultivable capability compared to the conventional land plant BECCS. Therefore, microalgal species are cultivated on a pilot scale in photobioreactors and ponds. In these contemporary days of global warming, microalgae are subjected to temperatures exceeding the optimal growth temperature, limiting the growth and yield. Respective adaptations of photoautotrophic algae to elevated temperatures act as a crucial factor for productivity (in terms of photosynthesis) as well as ecosystem stability. Therefore, mastering the evolutionarily conserved adaptations of photosynthesis is especially significant in the context of the current scenario. Since stress tolerance is a highly conserved process, it requires the coordination of several regulatory networks and multiple pathways. Recent studies reveal that stress response in Chlamydomonas was driven mainly by the composite, integrated network of transcription factors (TFs) to mitigate the stress effect because all the metabolic machinery expressions were under transcriptional control [73]. Thus, candidate transcription factors and their contribution to acclimatory response during high temperatures could be achieved by studying the TF mutants. Understanding these acclimatory responses and various physiological pathways under high temperatures at a molecular level will provide great insight into generating genetically engineered varieties of stress-tolerant strains. Besides these natural acclimation responses, microalgal strains with beneficial stress tolerance traits have been developed through gene manipulation techniques like CRISPR/Cas9, TALEN, etc. This review discusses some of the photo-physiology and CCM genes that are reported to be immune to acceptable high temperatures, which were identified by photosynthetic mutant cell studies. However, knowledge of how the complete photosynthetic light and CCM mechanism acted against a high-temperature background was still scanty. Hence, continuous screening of temperature-sensitive photosynthetic mutants would probably help find the composite relationship between photosynthetic components and their subsequent response to temperature stress. This would probably enhance our knowledge of the regulation of genes from a temperature perspective at the molecular and cellular levels. To develop genetically engineered thermotolerant plants, studying the protective mechanisms that enable the plants to respond to high temperatures is essential. Investigating the fundamental temperature stress-responsive system at different carbon dioxide concentrations in the plant model Chlamydomonas provides valuable insights into the heat stress-mediated regulation of the carbon fixation mechanism.
Future Perspectives
Chlamydomonas is a suitable model organism for studying the system-wide changes that occur during various environmental stresses. Recent advances at the molecular level have provided significant insights into the mechanistic detail of heat stress response and CCM. However, there is a lack of detailed information regarding carbon uptake, transport, and other cellular metabolic interactions at different temperatures. Therefore, further research is needed to provide a comprehensive understanding that could address this gap. Below are some questions that future research should aim to answer:
1. What would be the response of cells grown under photoautotrophic conditions at high temperatures and high CO2 stress?
2. CMM’s complete molecular mechanistic role under both high temperatures and high CO2 conditions needs to be unearthed.
3. How does HSR regulation occur when cells are subjected to high temperature and high CO2 stress?
4. It is unclear what the role of HSR/HSP in CCM regulation during high-temperature and high CO2 conditions is in obtaining tolerance to both stresses.
5. Which one of the calcium, TRP, and CNGC channels is primarily involved in the Ca2+ influx? Although the opening of the TRP1 channel depends on temperature, the influx of calcium through this channel has been understudied.
6. Since Ca2+ is involved in sensing both CO2 and temperature stress, how does the Ca2+ signaling mechanism mediate the CCM gene regulation and HSR during both heat and carbon stresses to be unearthed?
7. How does the interaction of different environmental stresses with high temperature influence CCM, and how do the HSPs interact with CCM regulation?
8. At high temperatures, the solubility of CO2 decreases in water. When high temperatures and high CO2 are applied to cells, how do the cells grow, and what changes occur in photosynthetic activity as well as carbon acquisition mechanisms in the cell?
9. Usually, in Ci stress conditions, carbon shifting occurs from carbohydrates to lipids before the complete activation of CCM in the cell. How does the mechanism of lipid metabolism regulation act when the cells are subjected to various carbon concentrations at high temperatures?
10. How does the interactive effect of CO2 and temperature stress influence lipid metabolism? Interaction between CCM and lipid synthesis under both stresses needs to be unearthed.
11. At high temperatures, remodeling of membrane lipids and accumulation of lipid droplets occur in the cell. Does the remodeling pathway in the above condition differ from the different Ci concentrations? Also, how does the mechanism of remodeling take place during both stresses? How does thylakoid membrane lipid remodeling influence CCM?
12. The influence of the interactive effect of high temperature and CO2 stress on fatty acid metabolism in biofuel production has to be cleared. Understanding these mechanisms will enable the unfolding of relevant strategies for application in biofuel production and CO2 mitigation.
13. How do the mutant cells regulate CCM at high temperatures? Unraveling the molecular-level changes in these mutants can help develop thermotolerant strains with effective CCM.
14. A multi-omics study may provide insight into interactive changes associated with CCM and other metabolisms at high temperatures and CO2 stress.
15. More research is needed to engineer heat stress-tolerant CCM in land plants.

