

Introduction
As an important component of forest ecosystems [1-3], headwater streams are widely distributed in forests, regulating the storages and fluxes of carbon and nutrients [4, 5] and playing a key role in the ecological safety of downstream aquatic environments [6, 7]. Because of the dense canopies of riparian forests that limit the input of light, headwater streams are characterized by low primary productivity [8, 9]. As a result, the input of allochthonous organic matter such as plant litter is the main source of carbon (C) and nutrients for the heterotrophic organisms in headwater streams, making plant litter one of the main carriers of the storage and migration of stream C and nutrients [10, 11]. Therefore, an increasing number of studies have studied the dynamics of plant litter in forest headwater streams [12, 13]. However, most of the studies have mainly focused on plant litter decomposition and the associated element release patterns [14, 15], and we know little about the dynamics of plant litter associated element storages, especially for those such as potassium (K), in headwater streams, which have limited our comprehensive understanding of the role of headwater stream in nutrient storage and migration.
Potassium is one of the macronutrients necessary for plant growth and development [16], participating in many biochemical and physiological processes of plant growth, such as osmotic balance maintaining, stomatal activity regulation, and promotion of the synthesis and transportation of organic substances [17, 18]. In general, the release of K during litter decomposition is one of the major sources of K in forest headwater streams, and the storage of plant litter K would thus significantly affect K cycling of the entire ecosystem. Plant litter K storage can be controlled by several factors that are tightly related to the input, output, and decomposition of plant litter, such as riparian forest type and the physicochemical characteristics of streams [13, 19]. For example, riparian forest types not only directly affect the input amount of plant litter [20, 21], but also the concentration of K in plant litter. Also, the quality of the inputted litter can affect litter K storage indirectly through controlling the release pattern of K associated with the litter decomposition process [22, 23]. Stream physical characteristics such as gradient, bank width, active channel width and water depth would also be important factors controlling the storage of plant litter K, because these factors can affect the distribution, output amount, and decomposition rate of plant litter [24], but have not been quantitatively assessed in the literature.
Stream water physicochemical characteristics would present another set of important moderator variables for the dynamics of litter K storage. For instance, the flow velocity and discharge of the stream can directly affect the input and output amount of plant litter and thus the associated litter K storage [25], and their effects on litter decomposition would regulate the release of K, contributing to litter K storage in headwater streams. Similarly, stream water temperature, pH, alkalinity, and dissolved oxygen are important factors for controlling litter decomposition process [26, 27], and would thus be important moderator variables for litter K storage in headwater streams. However, till now, we knew little about the dynamics of plant litter K storage and the associated drivers in subtropical forest headwater streams, and even less about the relative importance of different factors.
In this study, we continuously monitored the dynamics of K storage in plant litter as a whole and within different litter types (i.e., leaves, twigs, fine woody debris, reproductive parts, and barks) for one year in subtropical forest headwater streams, located in Sanming city, southeast China. We tested the dynamics of litter K concentration and the impacts of different factors on litter K storage, aiming to understand the underlying mechanisms. We hypothesized that (1) plant litter K storage in the headwater stream would be higher in the source than mouth reaches because of lower discharge and denser canopies of riparian forests in the source reaches; (2) stream litter K storage in the rainy season would be lower than that in the dry season because of larger litter output and decomposition rate; and (3) stream litter K storage would be controlled by several moderator variables such as the riparian forest type, stream characteristics, and water physicochemical characteristics.
Materials and Methods
Study Area
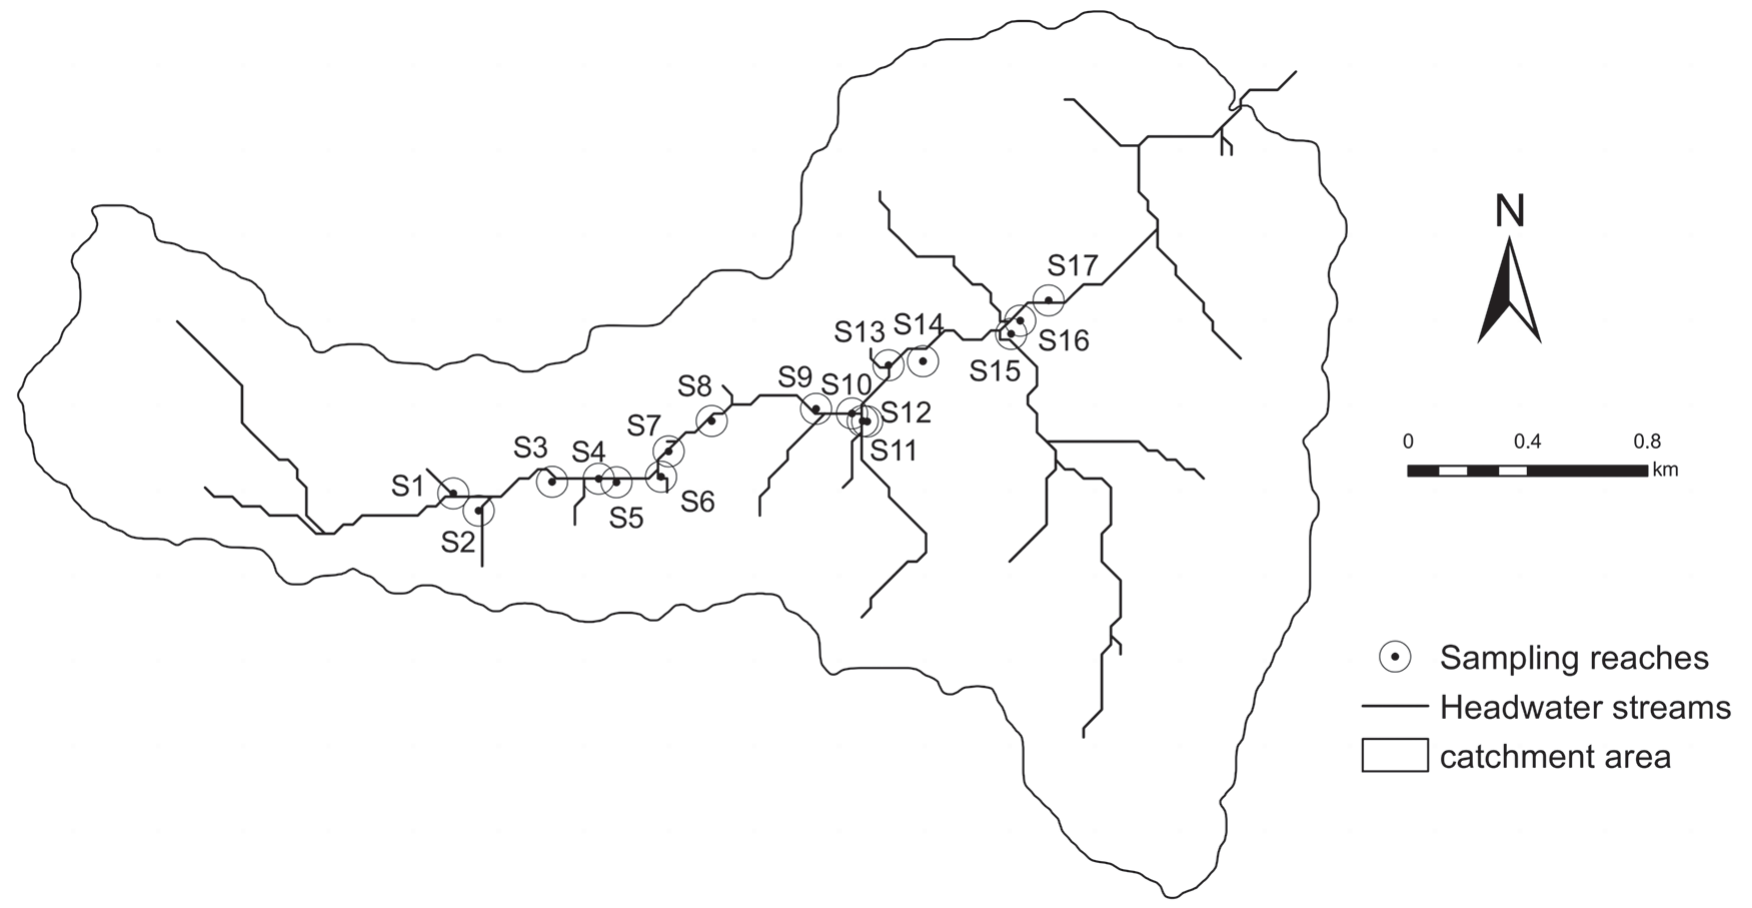
The study area is located at the Chenda Observation Site of the Sanming Forest Ecosystem Field Scientific Observation Research Station, Sanming city, Fujian province, China (26°19′ N, 117°36′ E). We selected a common headwater stream in the study area, which has a length of approximately 5 km (Fig. 1). The area of the catchment where the headwater stream is located is about 5.64 km2, and the terrain is dominated by low hills, with an average elevation of about 300 m. The region has a subtropical monsoon climate, with a long-term mean annual temperature of 19.3ºC and mean annual rainfall of 1,610 mm, and the majority of rainfall mainly concentrates between March and August. The main soil types in the study area are sandy red soils and yellow soils, and the nature of soil is acidic. The riparian forests of the stream are either dominated by Castanopsis carlesii (broadleaved forests) or by both Cas. carlesii and Cunninghamia lanceolata (mixed forests).
Field Aampling and Measurement
To monitor plant litter storage, we divided the stream into 17 sampling reaches from the source (S1) of the stream to mouth (S17). Because stream widths vary substantially among different reaches and the distribution of plant litter varies between the sides and middle areas, we thus set three sampling points at each reach with a sampling area of 1 m × stream width. Plant litter was sampled once a month from January 14 to December 25, 2021, at the end of each month. All the plant litter within each sampling point was collected by hand, and were then taken back into the laboratory for further analyses. A SL3-1 tipping bucket rainfall sensor (Shanghai Meteorological Instrument Factory Co., Ltd., China) was used to monitor the air-free rainfall data of the study area. Stream water conductivity, temperature, pH, alkalinity, and dissolved oxygen were measured within each sampling point for three times with a YSI-Proplus multifunctional water quality meter (YSI-Proplus, xylem, USA) at each sampling event. Stream gradient was calculated via ArcGIS 10.2, and stream bank width, active channel width, and water depth were measured with a tape. We also measured stream flow velocity with a portable flow meter (LS1206B, China) for three times at each sampling event, and calculated the corresponding discharge, and recorded if there is a tributary at each sampling reach.
Laboratory Analysis
The sampled plant litters were first cleaned with deionized water to remove surface silt and impurities, and were then air-dried. The air-dried samples were sorted into leaves, twigs (less than 1 cm in diameter), fine woody debris, reproductive parts (flowers and fruits), and barks. The sorted plant litter samples were then oven-dried at 65ºC to constant weights, weighed, and then ground to pass through a 60-mesh sieve for the determination of K concentration. The concentration of K was determined using an inductively coupled plasma mass spectrometer (ICP-MS, ULTIMA-2, JA, France).
Statistical Analysis
To evaluate if plant litter K concentration and storage varied among different sampling reaches (sampling time), we used linear mixed-effect models by fitting sampling time (sampling reach) as a random-effect factor. The effects of different moderator variables (e.g., riparian forest type, stream characteristics, and water physicochemical characteristics) on plant litter K storage were assessed using a linear mixed-effects model, in which we fitted sampling time as a random-effect factor and each variable as a fixed effect factor. Each moderator variable was assessed individually. For variables that showed a significant effect on plant litter K storages, we used a linear mixed-effects model selection method with the glmulti package using the great likelihood estimation to explore the relative importance of these variables [28]. The significance of each predictor variable is estimated based on the sum of the Akaike weights of all models that include that variable [29]. Based on previous studies, a threshold value of 0.8 was set for the Akaike weights to determine the most important predictors of K storage in plant litters [15]. All statistical analyses were performed in R version 4.1.3 [13].
Results
Spatiotemporal Dynamics of Plant Litter K Concentration and Storage
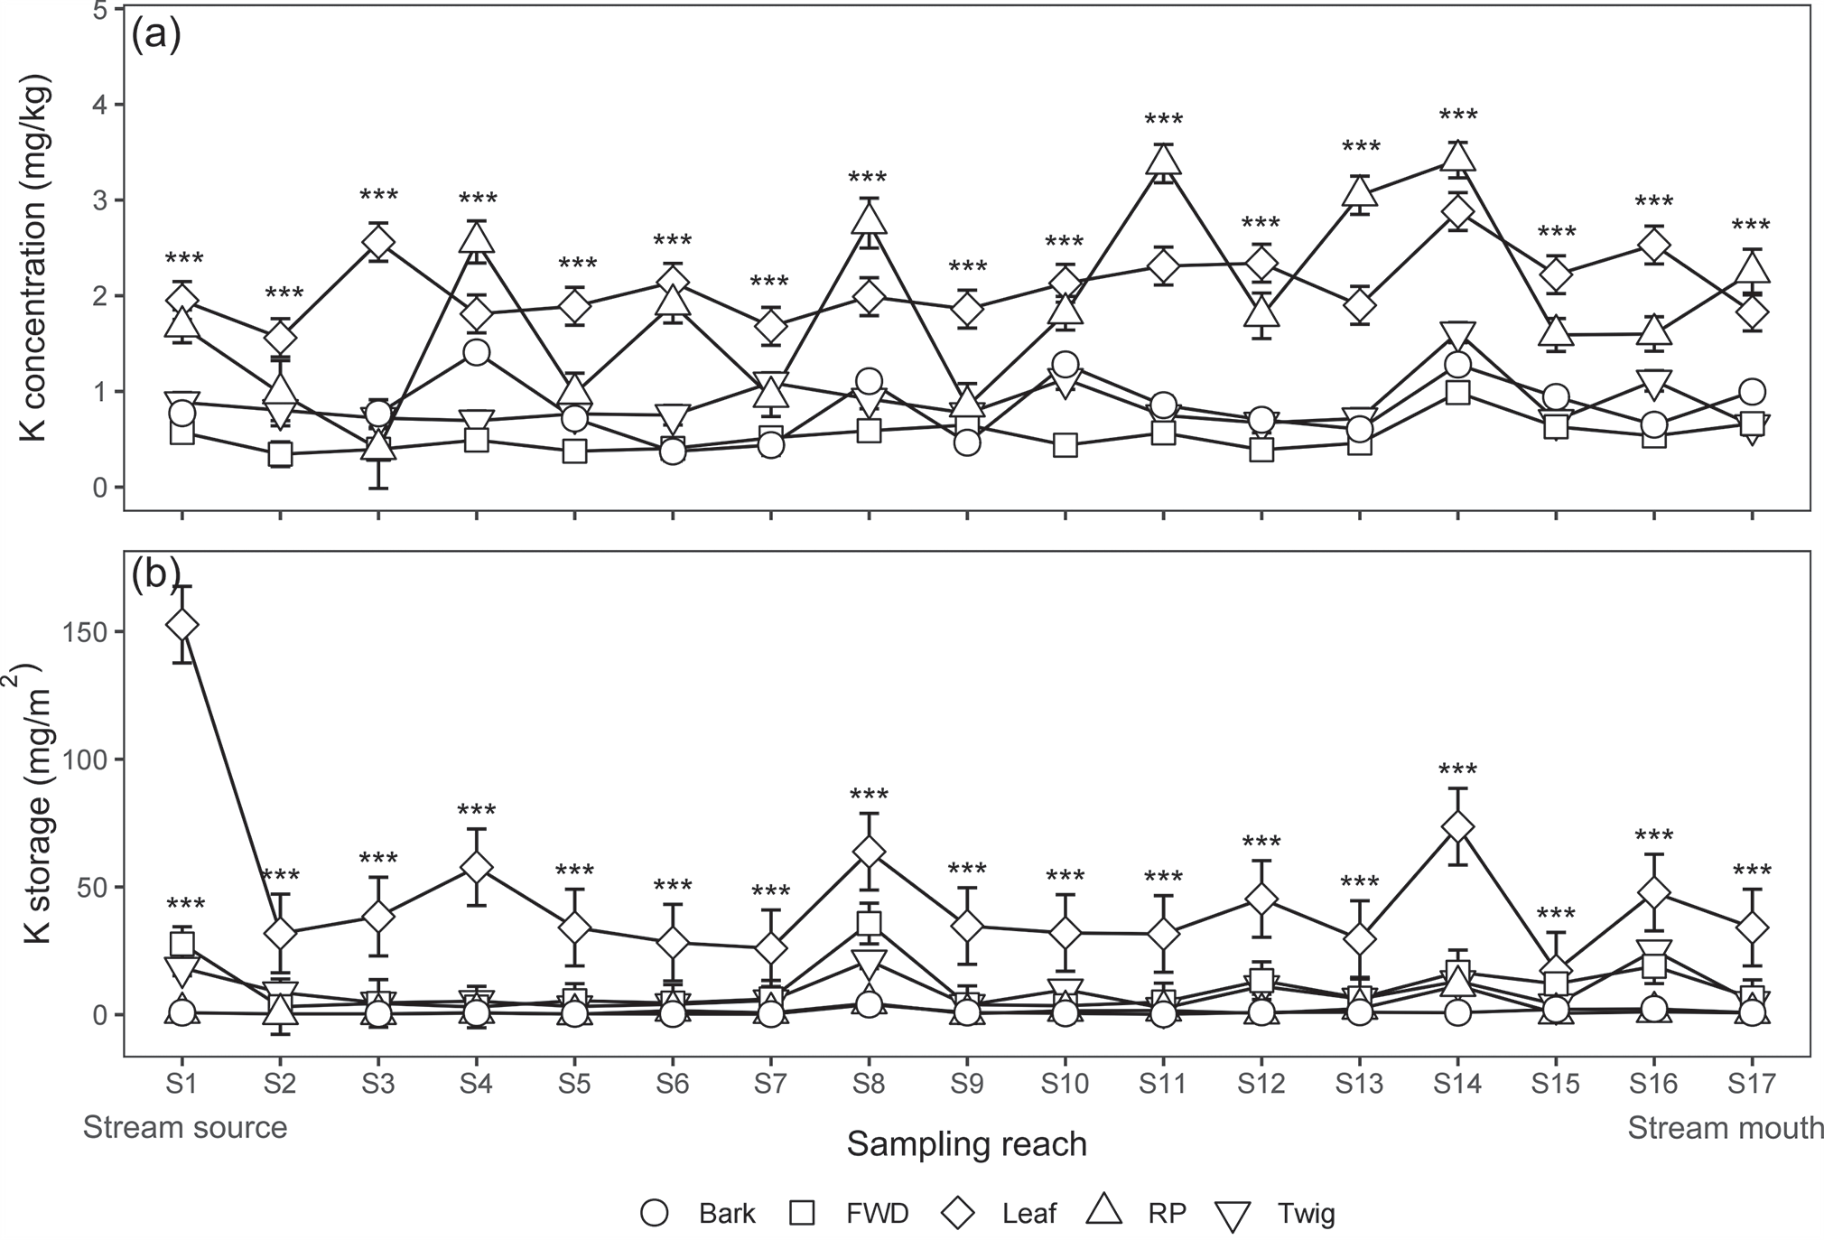
The annual average concentration and storage of litter K in the headwater stream were 1.4 mg/kg and 19.6 mg/m2, respectively (Fig. 2). Litter K storage showed an overall decreasing trend in the experimental year. During the dry season, litter K storage was relatively small with little fluctuations, while K storage of leaf litter, twigs, and fine woody debris peaked in April, and showed an increase-decrease pattern in the rainy season. Among different sampling reaches, litter K storage was highest at the source reach (S1), and K storage of litter leaves, twigs, and fine woody debris all showed a decreasing trend from the source to mouth reaches, while litter K storage of reproductive parts and barks did not show an obvious pattern among sampling reaches (Fig. 3).
Fig. 2.
Temporal dynamics of plant litter K concentration and storage in the forest headwater stream(mean±standard error, N = 3). Asterisks indicate significant differences among different organs in the same sampling month (*p<0.05, **p<0.01, ***p<0.001). FWD: fine woody debris; RP: reproductive parts.
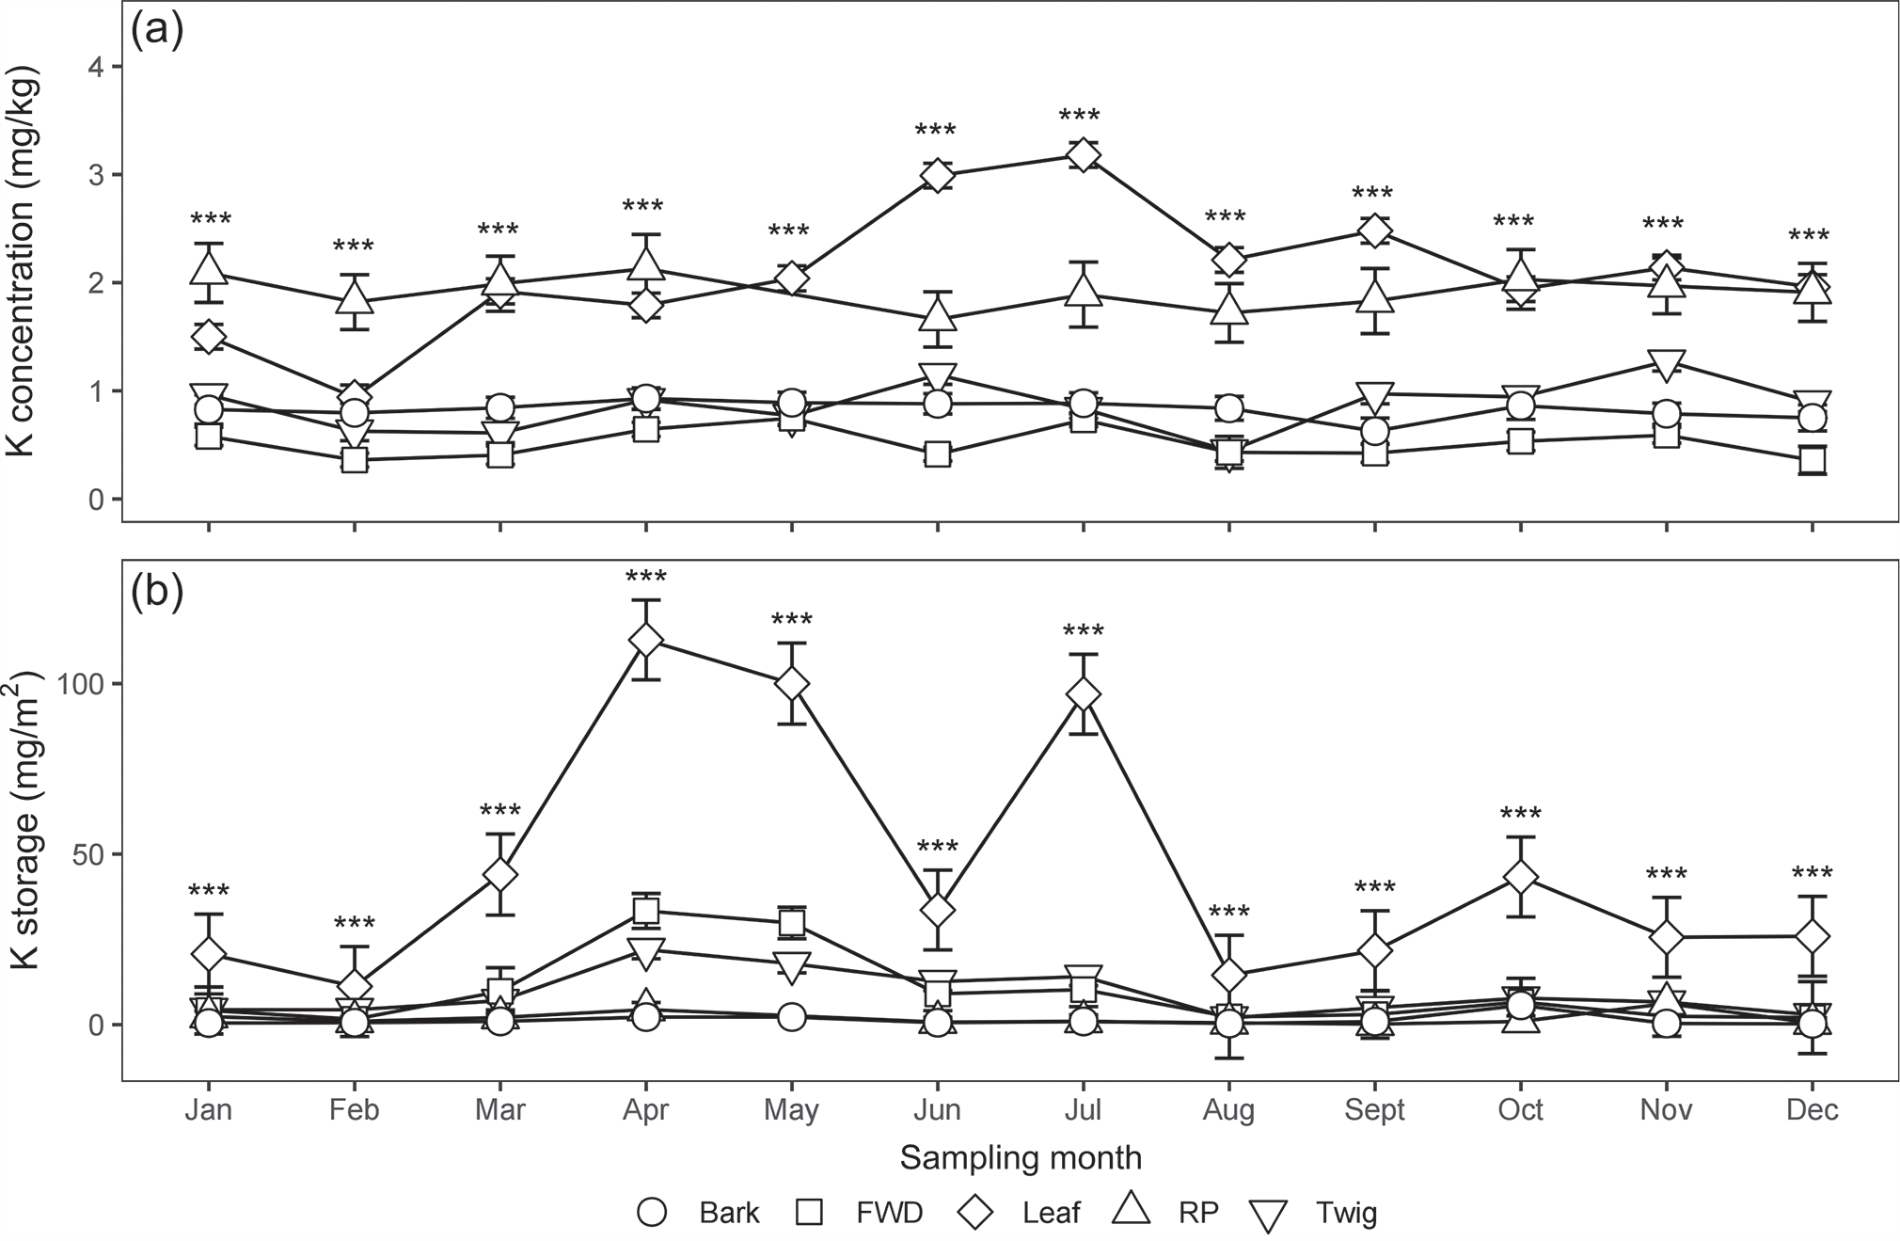
Fig. 3.
Spatial dynamics of plant litter K concentration and storage in the forest headwater stream (mean±standard error, N = 3). Asterisks indicate significant differences among different organs in the same sampling reach (*p<0.05, **p<0.01, ***p<0.001). FWD: fine woody debris; RP: reproductive parts.
Factors affecting litter K storage
Plant litter K concentration and storage were significantly affected by litter type, and the concentrations of leaves, twigs, and fine woody debris were 2.1, 0.9, and 0.7 mg/kg, respectively, and storages were 2, and 0.8 mg/kg for reproductive parts and barks, respectively (Fig. 4a). The total K storages of leaves, twigs, fine woody debris, reproductive parts, and barks were 45.7, 9, 12.5 1.9, and 1.4 mg/m2, respectively (Fig. 4b). The riparian forest type and the presence of a tributary only affected twig K storage, with higher storage in reaches with a confluence and under broadleaved riparian forests (Fig. 5). Leaf litter K storage was greater in reaches without a confluence, while K storage in twigs, fine woody debris, reproductive parts, and barks showed an opposite trend. Litter K storage in leaves, twigs, fine woody debris, reproductive parts, and barks were higher in reaches under broadleaved than mixed riparian forests, while leaf litter K storage was higher than in other plant litter (Fig. 5b).
Stream active channel width had a positive effect on K storage in leaf litter and fine woody debris, and water depth positively affected K storage in leaf litter and twigs (Table 1). Stream gradient had significantly negative effects on K storages of leaf litter, fine woody debris, and reproductive parts, while dissolved oxygen and alkalinity negatively affected K storage of leaf litter and twigs. Among the factors that significantly influenced K storage, rainfall and stream flow velocity were the most important ones for total plant litter, while stream water alkalinity and dissolved oxygen were the most important ones for twig and leaf litter (Fig. 6).
Discussion
In contrast to the hypothesis, our results showed that the maximum storages of K in leaf litter, twigs, and fine woody debris occurred in April, and the minimum storages in August. Climatic conditions, species, and decomposers are the main regulators of litter decomposition [30]. April and May are in the spring, the temperature rises, coupled with greater rainfall, the appropriate temperature and humidity will promote the emergence of leaves, the tree species will appear a short period of concentration of leaf replacement, the tree’s dead leaves will have a peak of fading [31, 32]. Also, streams have relatively high depths and flow velocity during this period, and plant litter is carried by streams to be stored within reach, which can also lead to peaks in plant litter K storage in streams [33]. In August, at the end of the rainy season, plant litter in streams undergoes predecomposition and fragmentation as they migrate downstream with flowing water, increasing the contact area of decomposers with plant litter [5], and combined with the fast rate of decomposition of plant litter in the aqueous environment, leads to a significant reduction in K reserves [34]. During the monitoring period, K storage of the leaf litter was higher than that of other types of litter, which may be that forest litter is mainly composed of leaves, and leaves are the most active component of the material cycle in forest ecosystems, with a shorter lifespan and rapid renewal, resulting in significantly higher leaf K storage than other organs [35, 36].
Among different sampling reaches, the maximum storage of leaf litter K occurred at the source reach (S1) of the headwaters stream, while the peak storage of K in fine woody debris, twigs, flowers and fruits, and bark occurred at the middle sampling reach (S8). Leaf litter K storage confirmed the hypothesis that the K storage of plant litter in the headwaters stream was greater at the source sampling reach than other reaches. The highest litter K storage may be attributed to the relatively low stream flow, scouring force and transport of the water body in the source sampling reach [37]. Coupled with the high density of riparian forest canopy, a large amount of leaf litter accumulated within the section of the stream, leading to a relatively high K storage [5, 38]. The peak of K storage in fine woody debris, twigs, and barks appeared in the middle reaches may be because the riparian forests of the middle reaches are dominated by Castanopsis carlesii with dense twigs and leaves, and more apomictic storage [39]. Also, compared with the other reaches, the reach is longer, with a gentler slope, and slower water flow rate, and the storage of plant litter would thus be large.
Fig. 4.
Characteristics of mean concentrations and storages of K in leaf, twig, fine woody debris (FWD), reproductive parts (RP), bark, and total litter (Total) in the forest headwater stream.
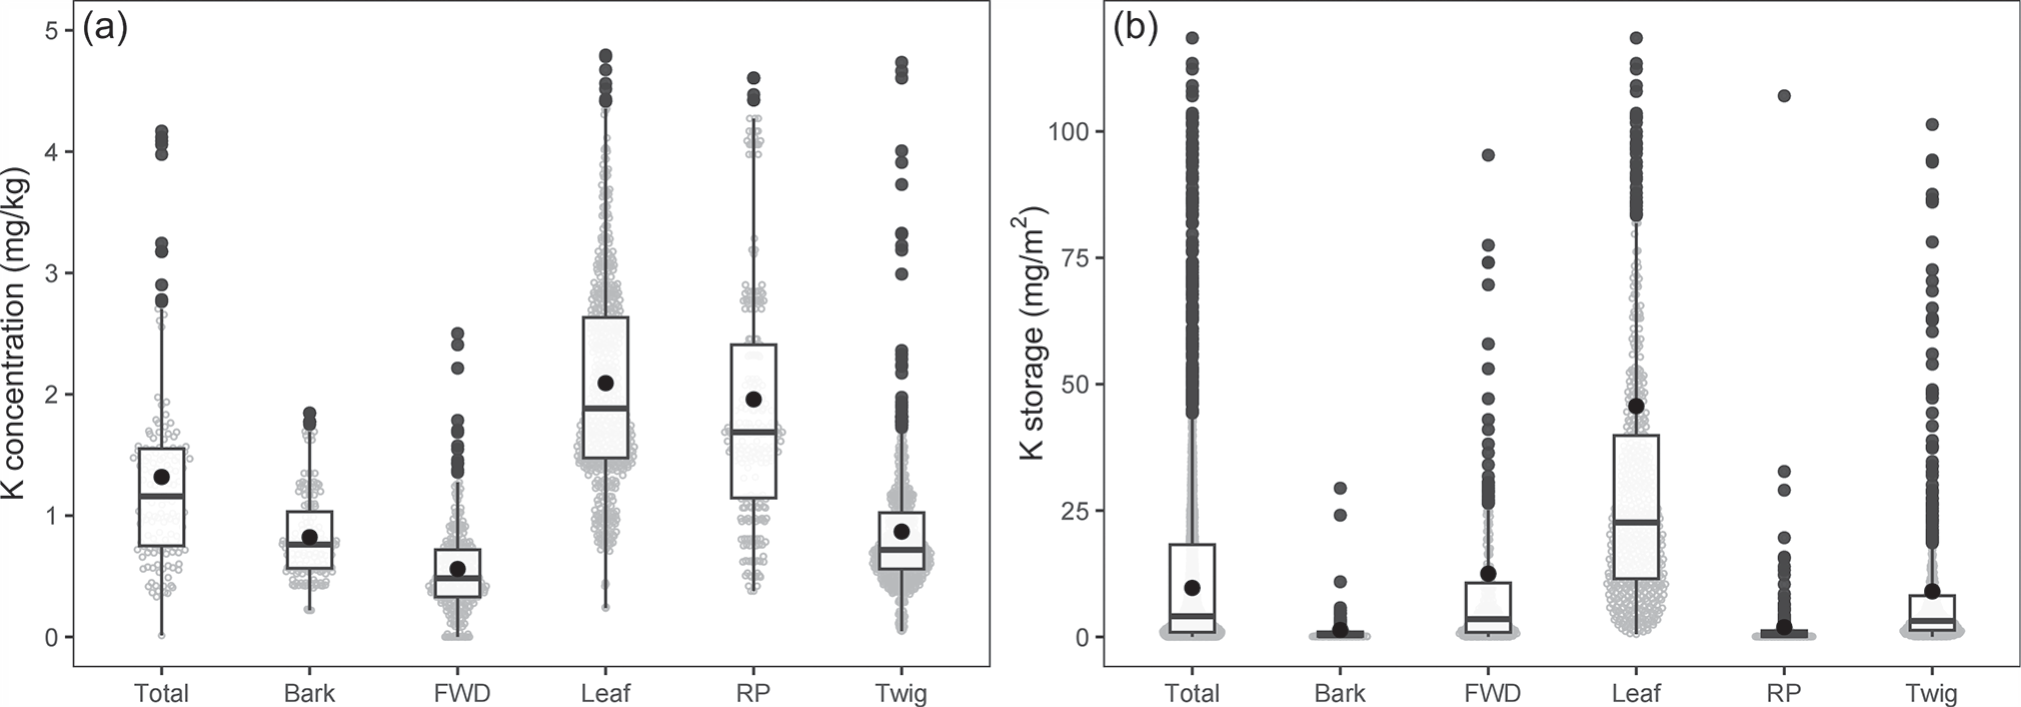
Fig. 5.
Effects of tributary and riparian forest type on litter K storage in the forest headwater stream. Asterisks indicate significant differences between sampling reaches with and without a tributary, or between broadleaved and mixed forests (*p<0.05, ***p<0.001). FWD: fine woody debris; RP: reproductive parts. Total: total litter.
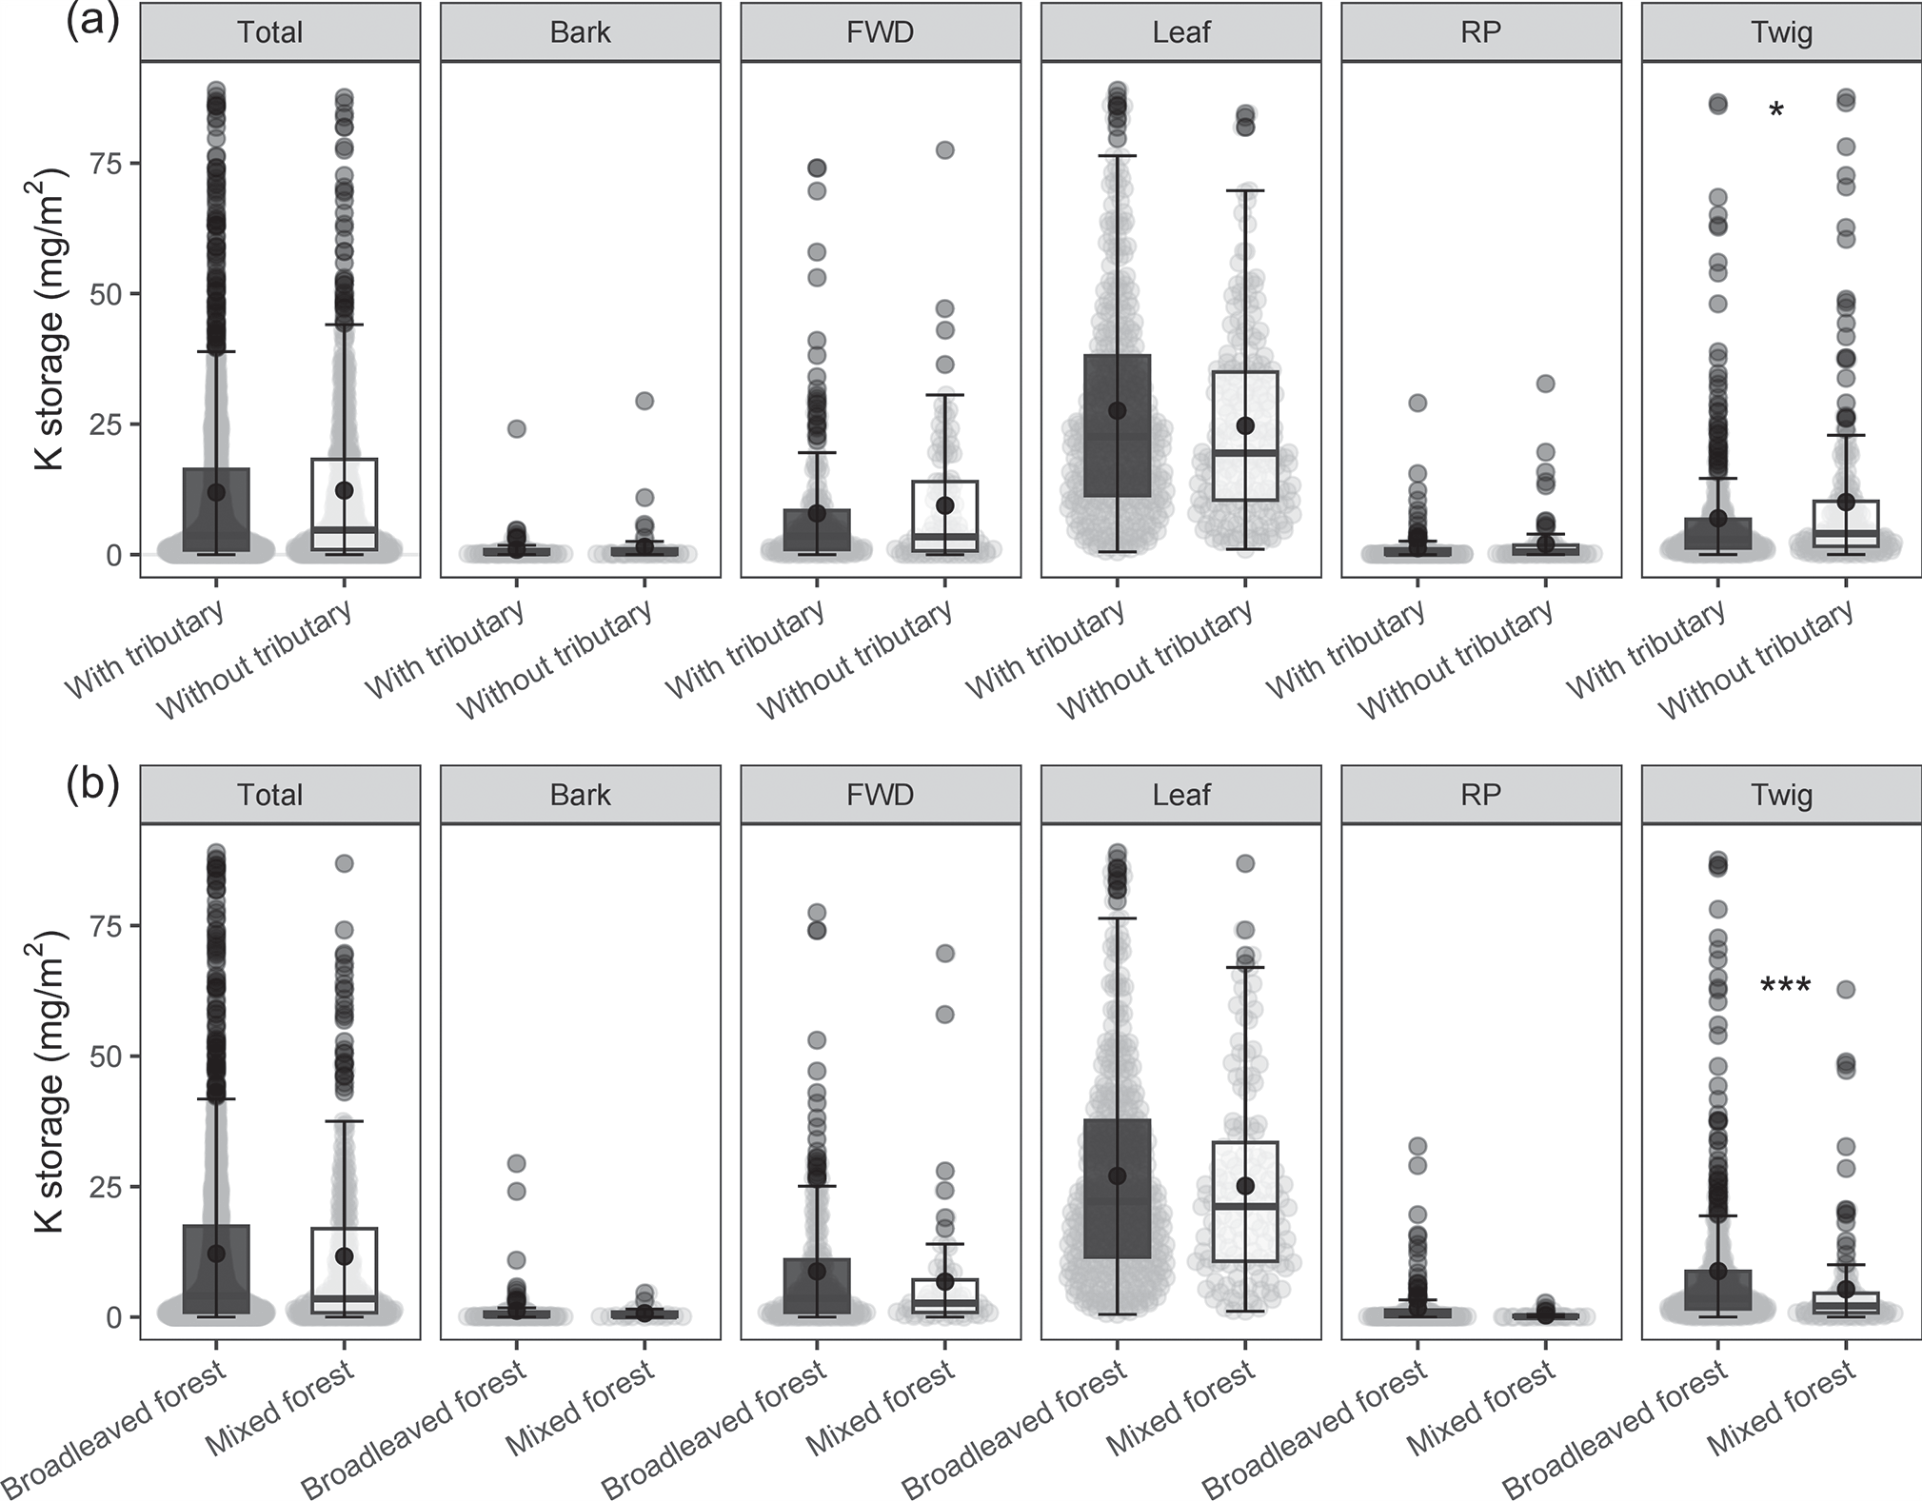
Fig. 6.
The relative importance of climate, riparian forest type, stream characteristics on K storage in total litter, leaf litter and twig as assessed using linear-mixed effect model selection method. DO: dissolved oxygen; ACW: active channel width; Tributary: the presence of tributary.
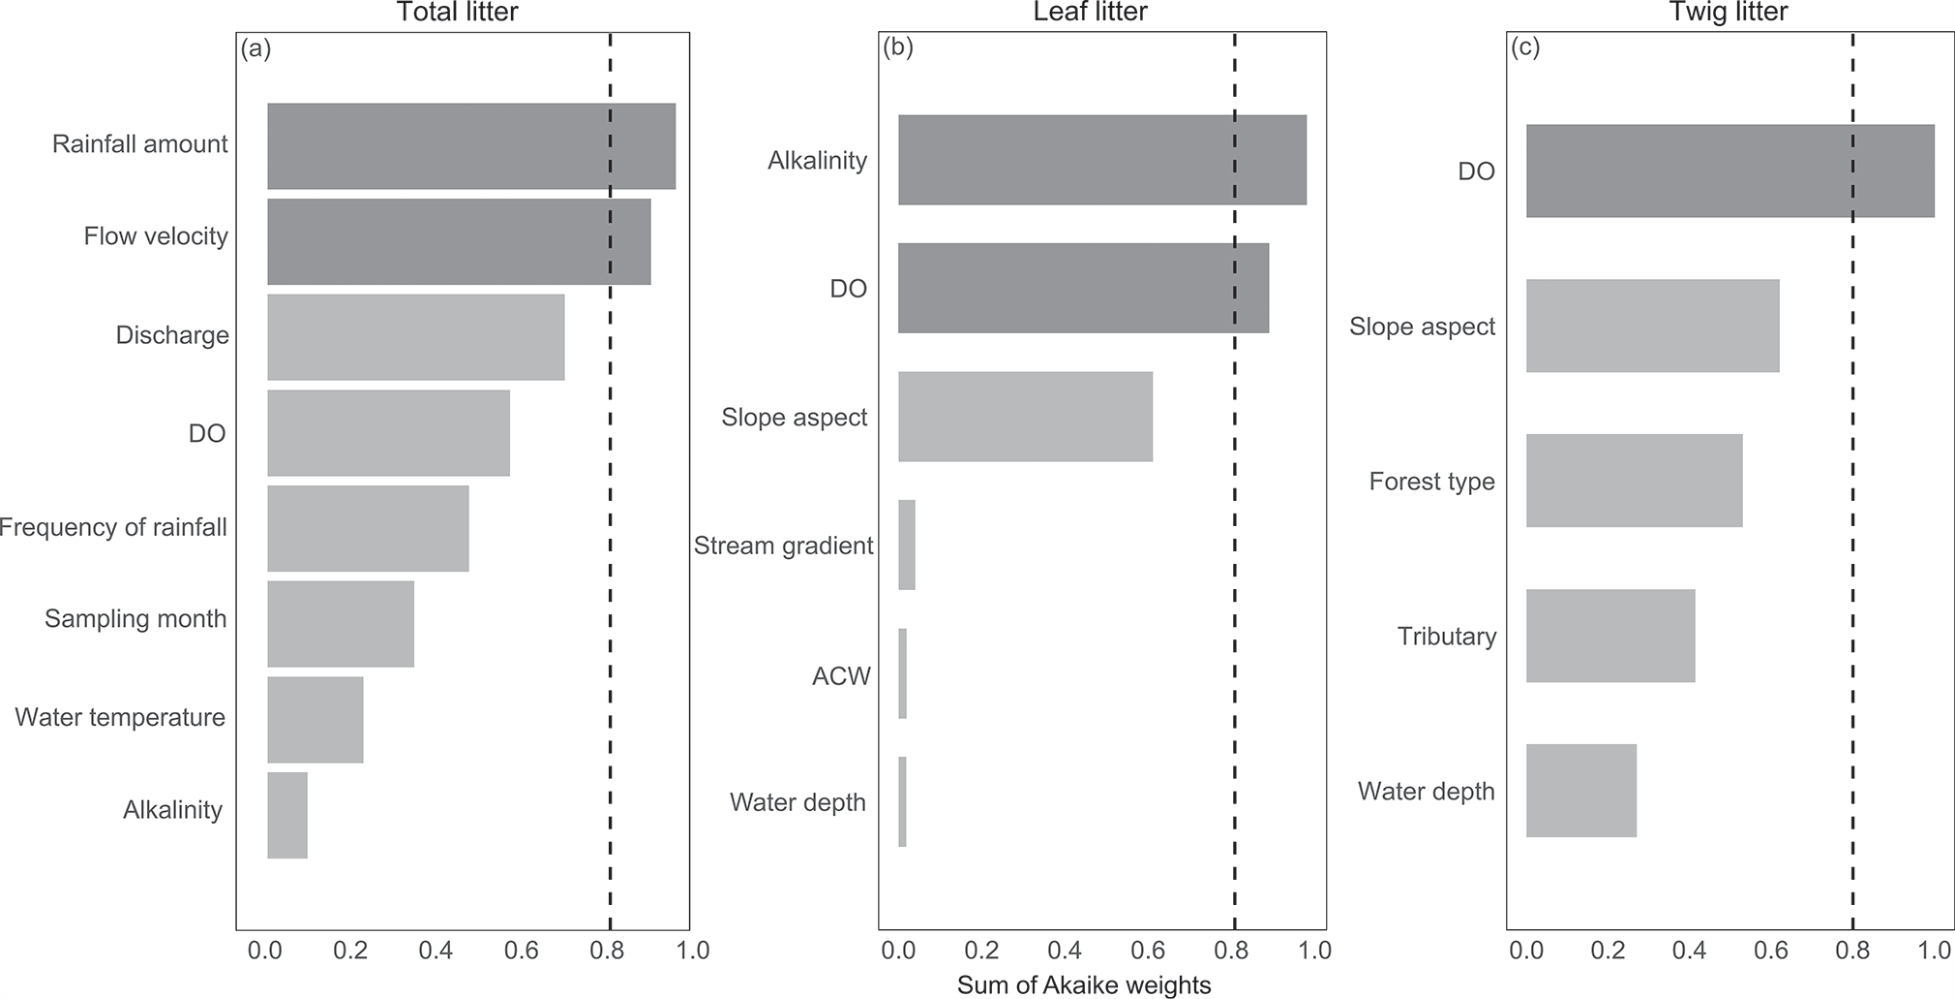
Table 1.
Effects of rainfall amount and stream characteristics on plant litter K storage as assessed using linear mixed-effect models. Estimates of the slope and the associated p-values are reported.
Leaf litter K storage is greater at the reaches without a tributary, because the tributary is a scouring zone, with alternating dry and tributary streams, with greater water scour, resulting in strong erosion of plant litter accumulating at the tributary and severe K loss [40, 41]. Also, the storage of K of other types of plant litter was greater at the reaches with a tributary, probably due to the fact that a tributary resulted in increased flow velocity and carried a high volume of plant litter [42], and that the water flows converge here to form the larger main stem, which has a large receiving surface for an apoplastic material. Litter K storage was higher in reaches with broadleaved riparian forests, which may be because of a higher K concentration and/or litter production of broadleaved forests compared to mixed forests.
We found that stream water depth had a significant positive effect on the storage of K in leaf litter and twigs, and the storage was greater in reaches with deeper water [43]. The width of the water was positively correlated with the storage K of leaf and fine wood debris, because the wider the water surface of a stream, the corresponding reduction in the velocity of the water and the scouring force, and the greater the width of the stream surface, the greater the area of reception of apomictic debris [44]. Stream gradient negatively affected K storage in leaf litter, fine woody debris, flowers, and fruits. In steeper gradient reaches, the scouring effect of water is greater, and plant litter is easily broken and decomposed, while plant residuals that are relatively light in mass are easily transported with water flow to the downstream reaches, thus affecting K storage [45, 46]. On the contrary, alkalinity and dissolved oxygen affect the decomposition of plant litter by influencing the microbial communities and activities of the stream, which can negatively correlate with K storage in apoplastic material [27, 47, 48].
Conclusions
Our results showed that the average annual concentration and storage of plant litter K in the stream were 1.4 mg/kg and 19.6 mg/m2, respectively, with an overall decreasing trend throughout the year. The peak of K storage occurred in April, while the minimum was in August. The peak of K storage appeared at the source sampling reach and the K storage of leaf litter, twigs, and fine woody debris showed a significant decreasing trend from the source to the mouth, with a decrease of 118.6, 13.4, and 20.5 mg/m2, respectively. Plant litter K storage was significantly affected by riparian forest type and the presence of a tributary, which was higher at reaches with broadleaved forests and without a tributary. Plant litter K storage is significantly influenced by stream water depth, active channel width, stream gradient, dissolved oxygen, and alkalinity. Overall, our study clearly indicated that plant litter in headwater streams can store a certain amount of K, and litter K storage has clear spatiotemporal heterogeneity. The results of the study can provide basic data and scientific bases for an in-depth understanding of nutrient transport and cycling along with ecohydrological processes in subtropical forest ecosystems.

