

Introduction
Pharmaceutical and personal care products (PPCP) have become an important issue in environmental toxicology because these chemicals cannot be removed from water through conventional methods. Thus, advanced oxidation processes, microalgal reactors, photocatalysis, among others, have been used to remove PPCP from wastewater [1]. It is estimated that their consumption, only in the United States of America, is about 10,000 tons per year [2]. Anti-inflammatory drugs are commonly used to treat pain and fever, inhibiting pathways like the synthesis of prostaglandins or enzymes like cyclooxygenases 1 and 2 [3]. Non-steroidal anti-inflammatory drugs (NSAID) like ibuprofen are prescribed under known commercial brands (like Advil®) in the case of transnational pharmaceutical companies and local brands (generics). However, painkillers can be purchased without medical prescription. Those active ingredients are then excreted almost unaltered, and in combination with some of their metabolites reach aquatic ecosystems through discharges from hospitals, as well as municipal and zootechnical facilities [4].
Ibuprofen (IBP) is commonly found in freshwater ecosystems, with a lifetime estimated at 4.6-32 d, and it is not affected by solar irradiance. NSAID is considered "biodegradable", but displays pseudo persistence due to its continuous release into the environment, caused by its high demand in human medicine [5]. IBP is metabolized to carboxyibuprofen, hydroxyibuprofen, and carboxyhydratropic acid, and approximately 15% of the total dose in humans is excreted without modifications, but conjugated with glucuronide and thiol [6]. Once in the environment, IBP-conjugates are hydrolyzed and produce diverse molecules in natural environments and wastewater treatment facilities [7].
Due to its continuous incorporation to water bodies, IBP has become an important issue for environmental research, considering this active ingredient to pose a potential risk for freshwater biota. Therefore, IBP is currently one of the most studied pharmaceuticals; generally, test organisms include cladocerans like Daphnia magna or another limnetic species like Moina macrocopa [8], some species of the genus Brachionus, and some other littoral species as representatives of rotifers and other invertebrates [9], and microorganisms, either autotrophic or eutrophic [10, 11].
While some mechanisms have been described with these test organisms, some environmental factors that modify the toxicity of IBP have not been fully explored. For instance, algal density is a main factor that influence the population performance of herbivorous zooplankters like cladocerans and rotifers; it is know that below certain algal density (incipient limiting concentration; ILC) cladocerans make an extra effort to acquire energy from the media through algae consumption, which implies a decay on filtering efficiency, and above the ILC, the movement of appendices decreases while the filtering efficiency becomes higher (higher energy obtainment) [12]. The threshold food concentration is an important concept in terms of individuals, as the amount of energy that shifts to maintenance (minimal metabolic rates) instead of reproduction; and in terms of population, as the minimal energy requirements to keep the growth rate at zero; and in general, larger organisms exhibit higher energy demand and food thresholds in opposition to smaller organisms that require less energy and possess lower food thresholds [13].
The ecological relevance of assessing the interaction of potentially toxic compounds and limiting algal concentrations relies on the constantly changing environments due to natural cycles, or on anthropogenic causes like the contamination-related decay of freshwater ecosystems, which can alter all taxa. Thus, algal cells might neither be at the same density and diversity, nor be of the same nutritional value, limiting filter-feeding organisms’ growth and reproductive performance. Therefore, this study aimed to assess the effects of the NSAID drug IBP on two freshwater zooplankton species, the cladoceran Alona gutta (Chydoridae: Aloninae) and the rotifer Lecane papuana (Monogononta: Lecanidae), cultured at three algal densities (0.25, 0.50 and 1.00 × 10⁶ cells/mL of Nannochloropsis oculata). We discussed the interaction of both factors, IBP and algae concentration, on the population growth of these two species.
Material and Methods
The strains of Alona guttata and Lecane papuana were provided by the Laboratory of Aquatic Toxicology of the Autonomous University of Aguascalientes. They both have been maintained in this laboratory for more than five years in moderately-hard reconstituted water (MHRW) (hardness: 80-100 mg/L as CaCO3; pH: 7.4-7.8), fed on the green alga Nannochloropsis oculata at 106 cells/mL, maintained at 25±2ºC, with a 16:8 photoperiod (light: dark) in a bioclimatic chamber (Revco Scientific, Inc.) [14].
Fifty to sixty parthenogenetic females of Alona guttata were placed in Petri dishes with MHRW and test organisms were obtained by daily separation of neonates (<24 h old) and placed in freshwater medium two hours prior to their usage. For Lecane papuana, 60 to 80 parthenogenetic females were placed in Petri dishes with MHRW and test organisms were obtained by daily separation of amictic eggs, which were placed in fresh MHRW without food supplementation, and kept at 25±2ºC until hatching.
Acute Toxicity Tests with Alona Guttata
Stock solution was prepared by diluting 200 mg of IBP in 10 mL of acetone (IBP 20,000 mg/L) that was used to prepare the test solutions, which consisted of at least five different nominal concentrations in a range from 10 to 100 mg/L. The highest concentration of acetone in the test vessels did not exceed 0.01% as recommended by the OECD guidelines, which represents a maximum amount of acetone 100 µL/L [15]. In addition, acetone has been tested as one of the less toxic solvents for zooplankton species [16].
The tests were performed in quadruplicate with 10 organisms (<24 h old) per replicate in a final volume of 2 mL in 24-well polystyrene microplates, which were then placed in an environmental chamber (Revco Scientific, Inc.) at 25±2ºC and at 16:8 (light: dark) photoperiod during 48 h. No food was supplemented during the test. The criterion for acceptance was at least 90% survival in the control group. Finally, mortality data recorded at the end of the toxicity tests (48 h) was used to estimate the median lethal concentration (LC50) through a concentration-response curve with the “drc” package of the statistical software R [17].
Acute Toxicity Assays with Lecane Papuana
The test solutions were prepared as aforementioned, and the range of concentration was set at 10 to 100 mg/L. The concentration of acetone did not exceed 0.01%, representing about 8 mg/L. For organisms of the family Lecanidae, acetone exhibits non-effect concentrations about 6000 mg/L [16]. Thus, that limit allowed us to estimate that acetone did not cause negative effects on the rotifers.
Then, ten neonates (<24 h) were placed in a well of 24-well polystyrene plate (Costar Inc.) for both controls and the different toxicant concentrations with a total volume of 1 mL. Rotifers were then transported to a bioclimatic chamber (Revco Scientific, Inc.), without food supplementation, for 24 h with a photoperiod of 16 : 8 h (light : dark), at 25±2ºC. After the exposure period the number of dead or immobilized animals was recorded. As a criterion of test acceptance, mortality in the controls was less than 10%. The LC50 values were calculated with the drc package in R [17].
Chronic Toxicity Tests with Alona Guttata
We followed the protocol described in [18]. Briefly, five cladoceran neonates (<24 h old) were placed in 2 mL of MHRW (negative control) or in one of five different concentrations (control, 0.40, 0.53, 0.80, 1.60 and 3.20 mg/L), which represent 1/160, 1/120, 1/80, 1/40, 1/20 of the LC50 for IBP. All treatments consisted of four replicas. Cladocerans were fed on N. oculata at: a) 0.25 × 10⁶ cells/L, b) 0.50 × 10⁶ cells/L, or c) 106 cells/L; kept at 25±2ºC, photoperiod 16 h : 8 h (light : dark), and a complete medium renewal was performed every other during 14 d (duration of the test). All experiments were conducted in 24-well polystyrene plates (Costar Co., USA). On daily basis, surviving females were counted while neonates were separated and counted, and fixed in formaldehyde (10% v/v) for further analyses. At the end of the test, adult females were fixed in formaldehyde. Then, neonates and adults were measured (length and width) with the aid of a microscope.
Data of survival (lx) and fertility (mx) were used to determine: average lifespan (D) (days), life expectancy at birth (ex) (days), generation time (G) (days), gross reproductive rate (GRR) (neonates/female), net reproductive rate (NRR) (neonates/female), and intrinsic rate of population increase (r, IRPI) (days):
The IRPI was computed through iteration with the Euler-Lotka equation:
Subchronic Exposure in Lecane papuana
Five different concentrations were assessed (control, 0.15, 0.30, 0.60, 1.21, and 2.42 mg/L, which correspond to 1/80, 1/40, 1/20, 1/10, and 1/5 of their respective LC50). Five rotifer neonates (< 24 h old) were placed in 2 mL of MHRW (negative control). Rotifers were fed on N. oculata at: a) 0.25 × 10⁶ cells/L, b) 0.50 × 10⁶ cells/L, or c) 106 cells/L; kept at 25±2ºC, photoperiod 16 h : 8 h (light : dark). Exposure period consisted of five days, and eight replicates per concentration were assessed. All experiments were conducted in 24-well polystyrene plates (Costar Co., USA). At the end of the incubation period, the number of individuals per well was counted and used to estimate the IRPI, using the formula:
where Nt is the final number of individuals, N0 is the initial number of rotifers, ln is the natural logarithm, and t is the exposure period (5 d).
Statistical Analyses
The LC50 values were estimated with the aid of the statistical package drc in R for Windows. Results of the chronic toxicity tests were analyzed through bifactorial ANOVA and Tukeys’s HSD multiple comparison test, where significant differences were established when P<0.05. For data visualization, plots were constructed with ggplot2 in R.
Table 1.
Results of the acute toxicity tests with Alona guttata and Lecane papuana exposed to ibuprofen.
[i] Note: * SEM, Standard error. LCx, Lethal concentration, concentration that affects 10 or 50% of the exposed population. LCx values were estimated with the aid of the statistical package drc in R for Windows. The equation corresponds to the log-logistic model with two parameters and correction for binomial data.
Table 2.
Estimation of the effective concentration for the intrinsic rate of population increase (IRPI) in Alona guttata exposed to Ibuprofen for 14 d and fed on Nannochloropsis oculata at three different algal densities.
Results and Discussion
Table 1 shows the results of the acute toxicity tests with both species. Alona guttata exhibited lower sensitivity to IBP than L. papuana; the LC50 value for the cladoceran was about 5 times higher than that for the rotifer. It is important to point out out that both organisms are considered littoral species, and that most of the studies performed with cladocerans and rotifers include planktonic species like Ceriodaphnia dubia, Daphnia magna, or D. pulex; and rotifers like Brachionus calyciflorus [9]. In this study, we included a chydorid, which is not commonly used in toxicity test protocols, but it could be a good representative of shallow water bodies, as could the littoral L. papuana [14]. Both A. guttata and L. papuana have been used in toxicity protocols and demonstrate their susceptibility to organic and metallic pollutants [18].
Daphnia magna is the cladoceran species most used in toxicity tests; thus, it is significant to establish comparison against their susceptibility. For IBP, Heckmann et al. [19] reported EC50 for immobilization at 108 mg/L and non-effect concentration (NOEC) at 40 mg/L, values that are superior to those found with the chydorid used in this study. On the contrary, Du et al. [20] reported that D. magna exhibited LC10 and LC50 at 11.9 and 23.5 mg/L, which could be explained due to interclonal differences in D. magna, both within and among commercial and laboratory strains [21]. In our case, we started the zooplankton cultures from a single female and propagated their progeny to diminish that effect; nevertheless, it is understandable that some variations might arise after several generations, but studying interclonal variation is beyond the aims of this research. However, we brought it to discussion as to identify whether this chydorid is or is not similarly sensitive to IBP in comparison to other zooplanktonic species.
In general, Lecane papuana has shown to be more tolerant than other rotifer species to some chemicals, including pesticides, although its susceptibility to pharmaceuticals is very similar to that of other species [22]. Literature reporting the effect of IBP on rotifers is still scarce. In the ECOTOX Knowledgebase with the query terms “Brachionus”, “ibuprofen”, “CAS 15687-27-1”, “rotifer”, “all endpoints”, and “all effects”, we obtained no more than 320 hits [23]. Several of this results included CAS numbers of other non-steroidal anti-inflammatory drugs (NSAIDS) like diclofenac, and steroidal compounds like 17β-estradiol, among others. Consequently, this study is a contribution to the knowledge about the toxicity of a commonly used NSAID toward the rotifers. González-Pérez et al. [24] exposed B. calyciflorus and B. havanensis to IBP sublethal concentrations, from 6.25 to 25 mg/L; however, such concentrations represent the interval used to estimate the LC50 for L. papuana (12.053 mg/L), which could be considered more sensitive to IBP.
Fig. 1.
Results of the subchronic exposure of Alona guttata to ibuprofen (IBP) and fed on three different algal concentrations of the green alga Nannochloropsis oculata (0.25, 0.50 or 1.00 × 10⁶ cells/ mL). Females chydorids were exposed for 14 days and all treatments were carried out by quadruplicate. D, average lifespan; ex, life expectancy at birth; G, generation time; GRR, gross reproductive rate; NRR, net reproductive rate; IRPI, intrinsic rate of population increase. Significant differences (P<0.05) were established through two way ANOVA and multiple comparison test of Tukey HSD. Statistical analyses were performed with the aid of the package agricolae and graphics were plotted in ggplot2, both in R for Windows.
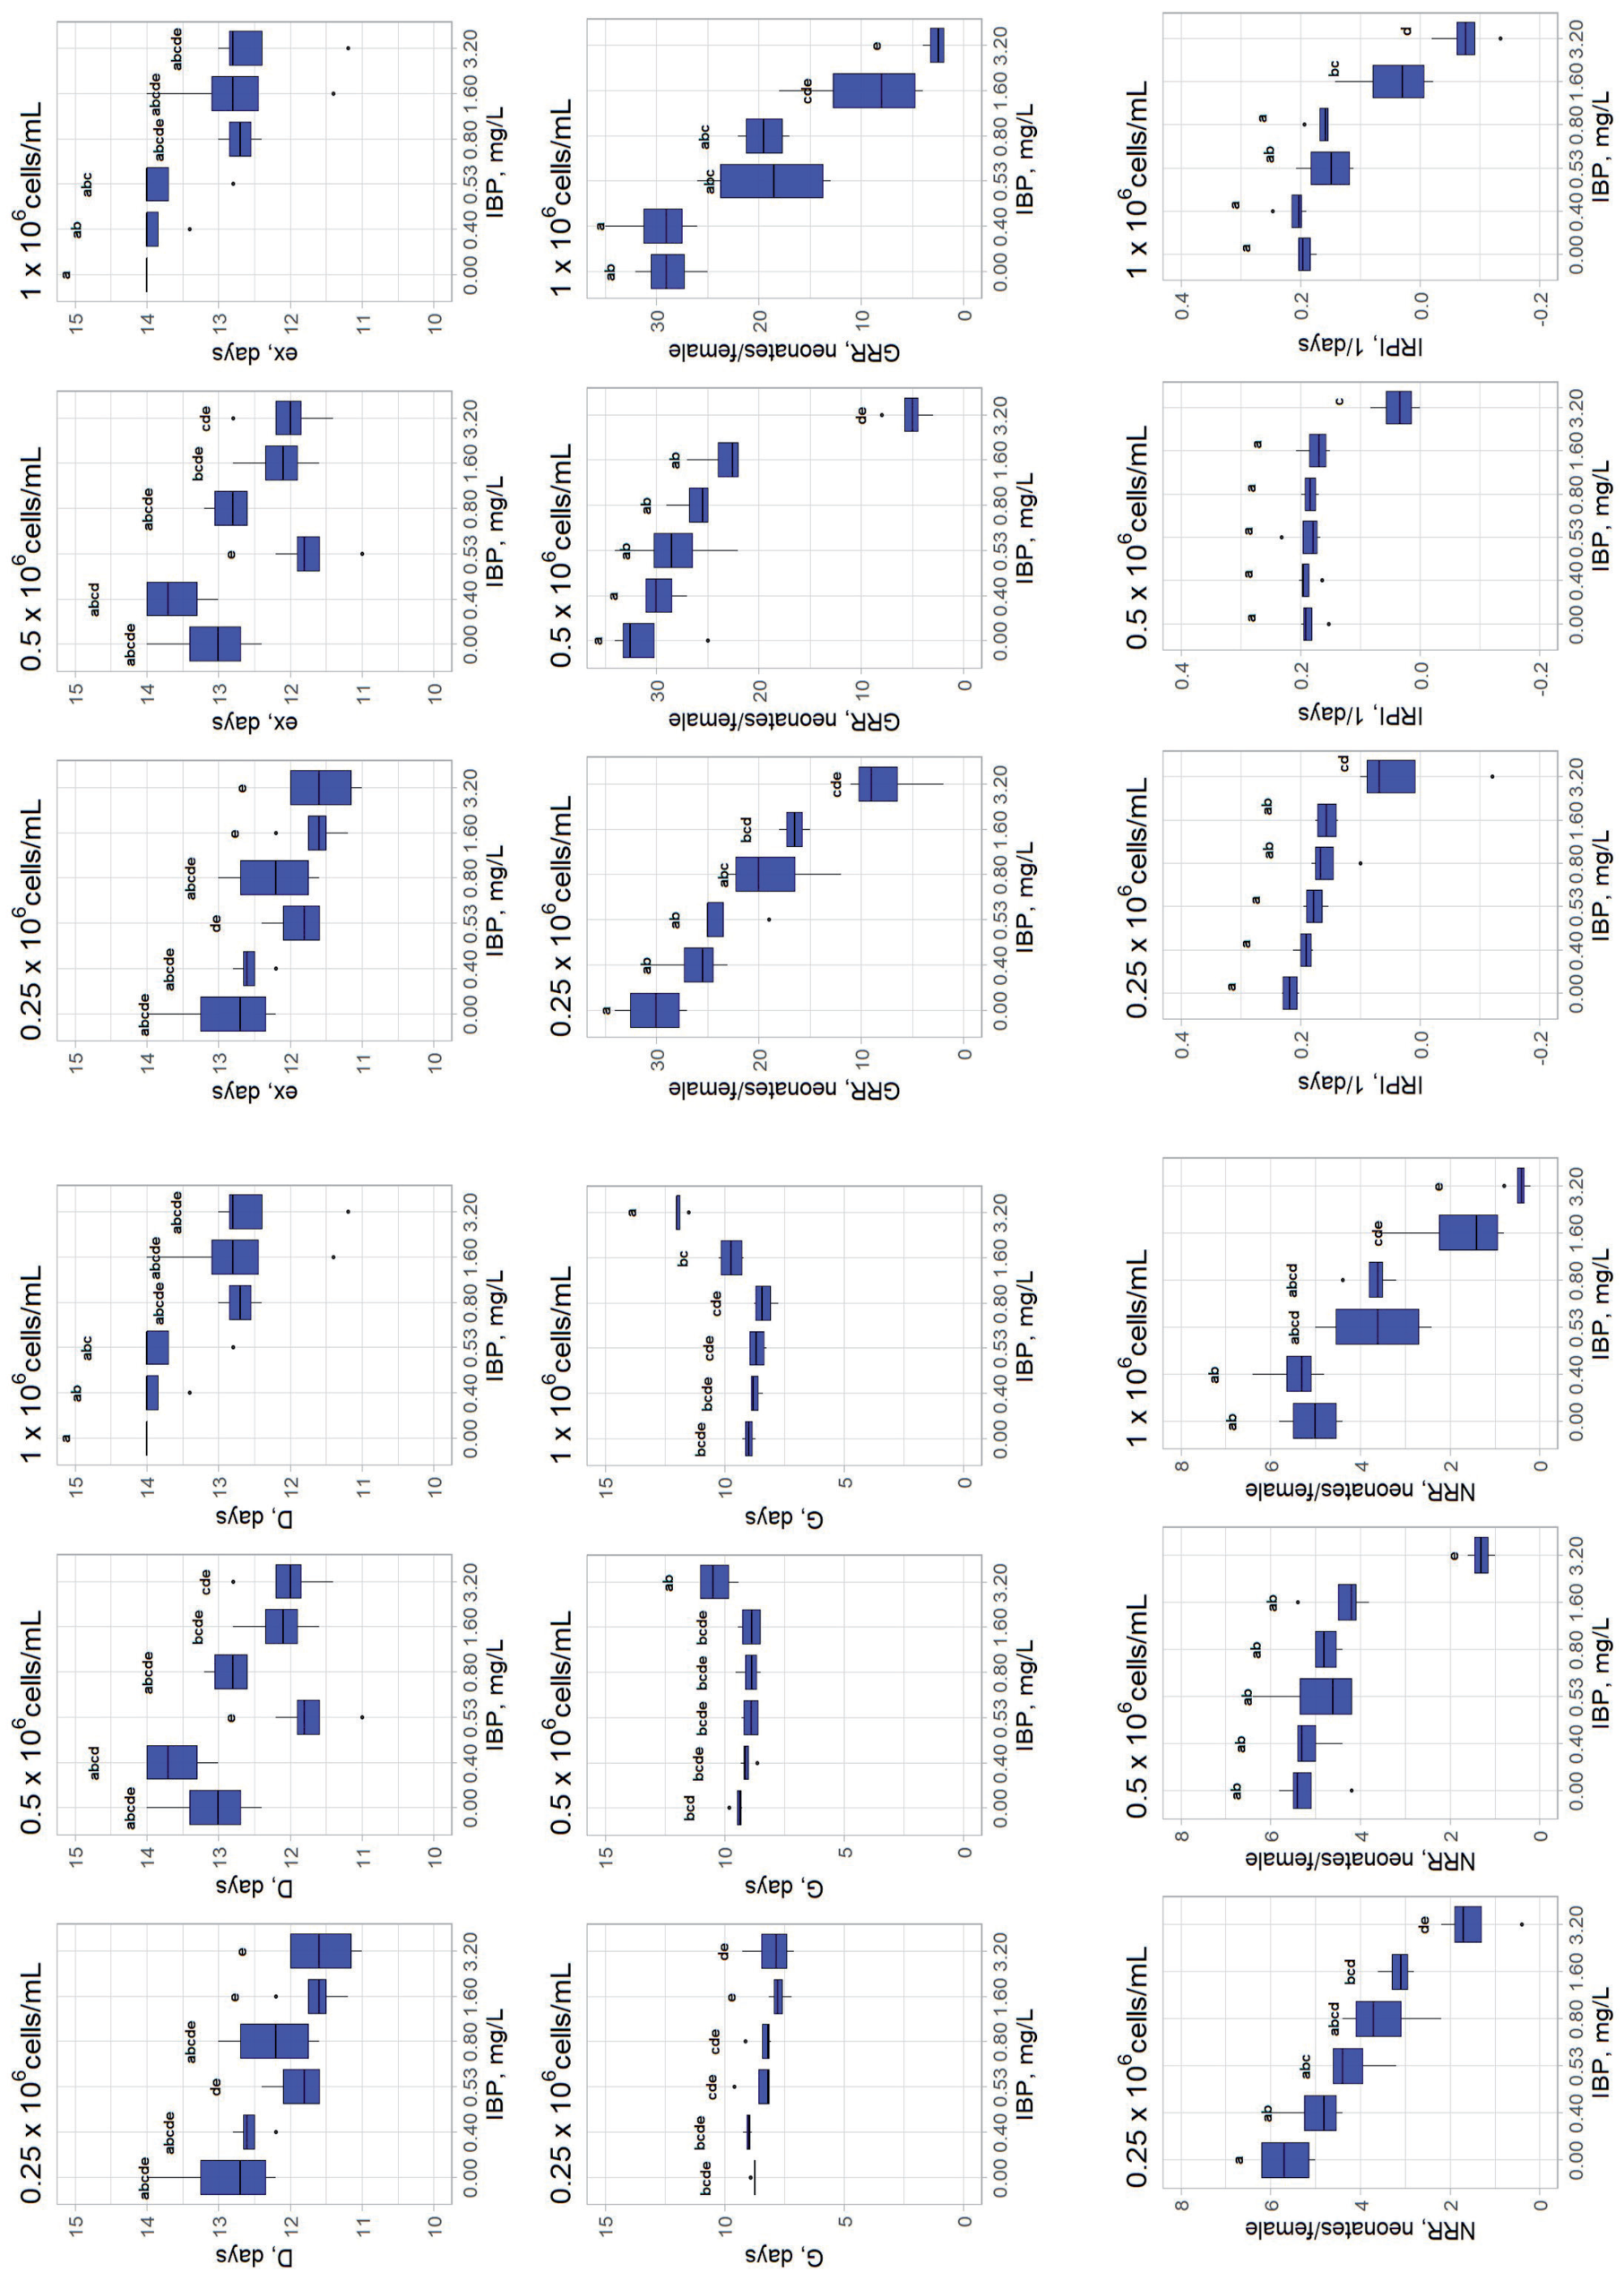
Table 3.
Estimation of the effective concentration for the intrinsic rate of population increase (IRPI) in Lecane papuana exposed to Ibuprofen for 5 d and fed on Nannochloropsis oculata at three different algal densities.
Zuriaga et al. [25] evaluated the acute toxicity of IBP toward Aliivibrio fischeri (Gram negative bacteria) and compared their results with those of previous studies with other taxa like D. magna and the microalga Raphidocelis subcapitata (formerly Pseudokirchneriella subcapitata). These authors discussed the classification of IBP in accordance to that one of Passino and Smith [26], which states that compounds with EC50 values from 10 to 100 mg/L can be considered as slightly toxic, while EC50s from 1 to 10 mg/L comprise moderately toxic compounds; thus, for both the species herein studied, IBP can be considered as a slightly toxic to A. guttata and L. papuana. However, such a classification is based on the LC50 values, and it changed from slightly toxic to moderately toxic when chronic responses were included.
The average lifespan (D), life expectancy at birth (ex), and the generation time (G) of A. guttata exhibited no significant differences when exposed to sublethal concentrations of IBP (0.40 to 3.20 mg/L) (Fig. 1). In addition, the algal density (0.25, 0.50, and 1 × 10⁶ cells/mL) did not alter these same population parameters. However, the gross and net reproduction rates (GRR and NRR, respectively) diminished at the two highest concentrations tested (1.60 and 3.20 mg/L). Due to the relatively high survival of Alona exposed to IBP and the alterations of the number of offspring per female, the intrinsic rate of population increase (IRPI) decreased in comparison with the control, but only at the highest IBP concentration. Apparently, algal density was not a factor to alter fertility and survival of A. guttata since no significant differences were found among the organisms fed those three algal densities.
Alona guttata in a 14-d period showed no significant changes in survival when fed on different densities of N. oculata, but was limited by temperature, with the best results at 25ºC. Therefore, we expected all controls to reach D values about 14 d, including those fed on 0.25 × 10⁶ cells/mL, and that mortality could be explained by the exposure to IBP. As seen in Fig. 1d), ex, and G were neither affected by the algal density nor by the IBP (except to the highest concentration tested). Probably, survival and fertility in A. guttata are improved by the inclusion of a substrate (sediment), which represents an extra input of organic matter that could be used as food source by the chydorids; consequently, the population performance of Alona was improved. In our study, artificial substrate was not included as it could adsorb the IBP and contribute (or not) to toxicity, which is not included in our aim to evaluate the effect of algal density and IBP concentration. Furthermore, subchronic toxicity tests with and without substrate addition showed no evidence of altering survival or fertility [27].
Our results are like those of Gu et al. [28], who used Moina macrocopa as test organism to assess the effect of IBP (0.45-14.4 mg/L) at three different algal densities (0.50, 1.00, and 2.00 × 10⁶ cells/mL). These authors described that IBP did not significantly affect the ex and GRR, while the NRR and survival exhibited lower values compared to controls. Nonetheless, all demographic parameters were influenced by the algal density, and not all of them by the interaction of both factors. However, the IRPI exhibited significant reductions in both studies, although the negative effects on chydorids were observed at lower concentrations than those of the cited report, which might represent higher tolerance of M. macrocopa to IBP.
Fig. 2.
Measures of Alona guttata exposed to IBP and fed on three different algal concentrations of the green alga Nannochloropsis oculata (0.25, 0.50 or 1.00 × 10⁶ cells/mL). Adults (left column) represent those organisms that survive after 14-d exposure. Neonates (right column) represent the organisms born from the exposed females. All treatments were carried out by quadruplicate. Significant differences (P<0.05) were established through two way ANOVA and multiple comparison test of Tukey HSD. Statistical analyses were performed with the aid of the package agricolae and graphics were plotted in ggplot2, both in R for Windows.
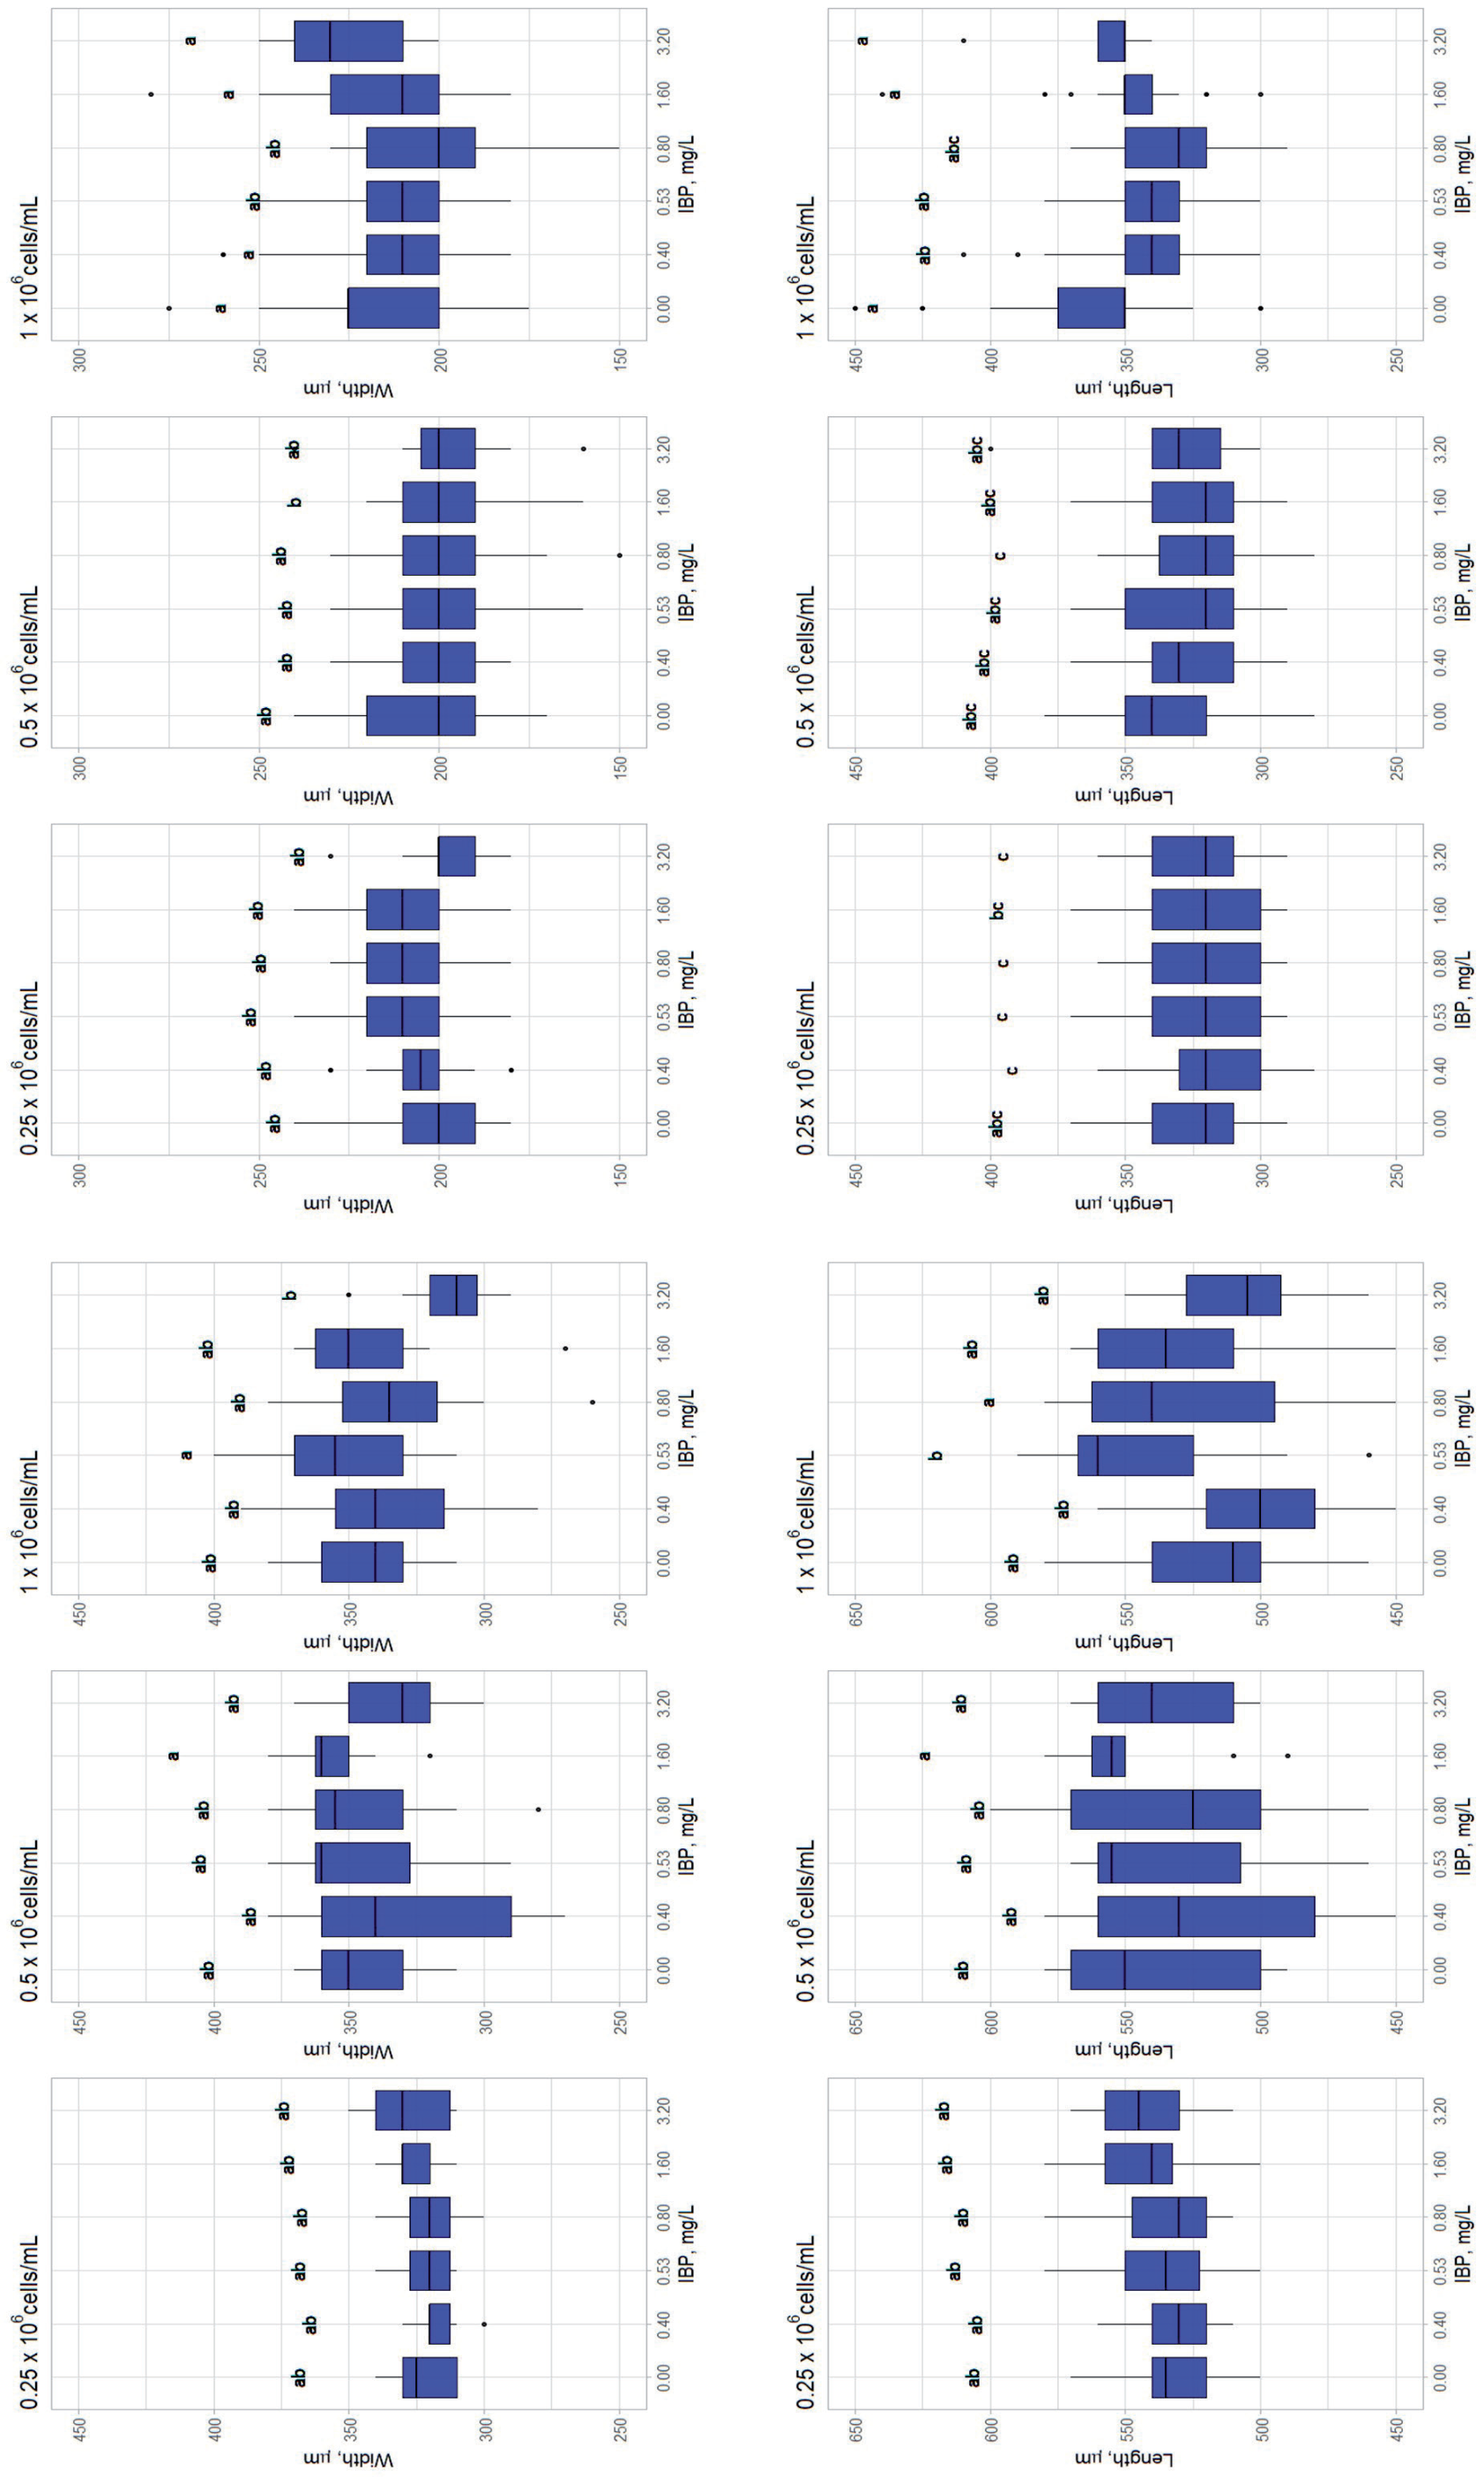
Fig. 2 shows length and width of adult females and juveniles of A. guttata, either from controls or IBP-exposed groups. There were no differences among the treatments, neither because of the algal density nor due to the IBP concentrations. Some authors have used the size of adults and neonates as endpoints to determine the effect of environmental conditions (including the exposure to toxic compounds) on the reproduction process [29, 30]. There is a generalized idea about the following trade-off in cladocerans: stressed daphnids shift from numerous clutches (quantity) to bigger size neonates (quality). When daphnids acquire more energy from the environment and there is no factor of stress, then, less energy is allocated to each egg that will turn into a smaller neonate; in contrast, low algal density or harsh environmental conditions cause daphnids to allocate more energy into fewer eggs that will become bigger neonates [31]. Therefore, we expected chydorids to follow the same pattern that daphnids did, but it is very likely that the same trade-off cannot be observed in Alona. We hypothesized that chydorids might have longer interbreed periods to accumulate enough energy to produce their offspring; thus, what we can observe is the reduction in the total offspring per female.
It is important to point out that the hypothesized mechanism opens new lines for further investigation, taking into consideration that biology of chydorids is not as known as that of other cladocerans families like Daphniidae or Moinidae, which might be due to the uneasy taxonomic work to identify Chydoridae:Aloninae specimens, and that some of them possess specific diet requirements. Osorio-Treviño et al. analyzed the effect of deltamethrin and lead (Pb2+) on the caloric content of adult females of A. guttata, but did not consider those same endpoints for the neonates, nor their size, born from stress mothers [18]. As above, maternal effect has been documented for species of the genus Daphnia; basically, daphnids, sensing stressful conditions in the environment, trigger some mechanisms to allocate more energy to fewer number of organisms within their clutches, the so-called shift from quantity to quality, conferring their offspring better chances to survive in the stressful environment [32-34].
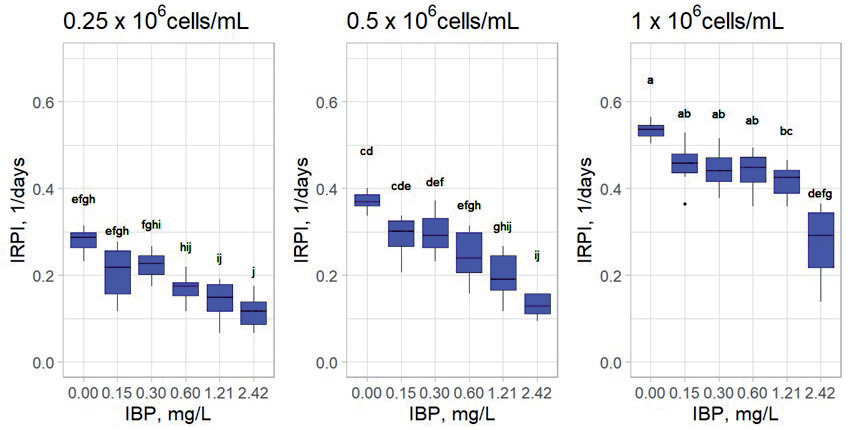
Fig. 3 presents the results of exposing L. papuana to sublethal concentrations of IBP (fractions of their respective LC50). In contrast to A. guttata, the rotifers exhibited decreased population growth, influenced by both algal density and IPB increasing concentrations. These data were used to estimate their EC50, which decreased in response to the algal density; the lower the algal density, the lower the EC50 of IBP for rotifers. The EC50 at 0.25 × 10⁶ cells/mL is about six times lower than EC50 at 1.00 × 10⁶ cells/mL (Table 3). This implies that algae density plays an important role in the effect of IBP toward L. papuana. Some authors have studied the effect of algal density and its influence on the toxicity of selected compounds [35-37]. Demographic parameters are affected by the algal density; in general, higher concentrations of algae enhance reproductive performance, but concentrations above 4 × 10⁶ cells/mL seem to elicit opposite effects, as well as low food concentrations.
Jiang et al. [38] examined the effect of algal density (1.00, 2.00, and 4.00 × 10⁶ cells/mL) and oxytetracycline on B. calyciflorus. Their results showed that increasing algal concentration stimulated the demographic responses of the rotifers, and that at low antibiotic concentration the population growth is higher than in controls, but increasing the antibiotic concentration inhibited fertility and survival. As in our study, the higher the algal density, the higher the population growth, and apparently, the toxicity of the pharmaceutical decreases.
González-Pérez et al. [24] exposed B. calyciflorus and B. havanensis to sublethal concentrations of IBP and fed them on a single concentration of microalgae; however, the concentrations used in that study are higher than those we used; they reported effects on concentrations above 6 mg/L, while we determined the EC50 at 3.097 mg/L when feeding at 1.00 × 10⁶ cells/mL; thus, L. papuana was 2 to 8 times more susceptible to IBP than the two Brachionus species.
Food supply in these experiments includes different microalgae species (which depend on the zooplankton species to be fed); however, all publications referred to using living algal cells (unless authors declared the opposite). Algal cells represent an energy source for cladocerans and rotifers, which require certain algal density to cover their energy needs: basal metabolism, individual growth, and reproduction; nevertheless, both extremes, limiting and excessive algal density can negatively affect population growth rates and performance, indicating that zooplankton species can grow within certain interval without significant differences [39].
Besides being an energy source for cladocerans and rotifers, algae biodegrade IBP and remove it from the medium [40, 41], but toxicity might not be reduced since IBP metabolites and intermediate compounds of IBP degradation are more toxic than the parent compound [5, 42]. IBP metabolites include hydroxylated compounds (OH-IBP) and carboxylic acid IBP (CA-IBP), which can be produced by bacteria and microalgae, and by physicochemical mechanisms like photolysis and advanced oxidation processes (AOP). Thus, biological and physicochemical alterations of IBP might expose chydorids and rotifers to a complex mixture of the parent compound and its metabolites. A possible explanation for the differences between A. guttata and L. papuana relies on the experimental setup. For cladocerans, complete media renewal was performed every two days, which represents a continuous supply of IBP despite its likely biodegradation and removal within some hours by algae-mediated mechanisms. However, removal of IBP and its metabolites could also be performed by absorption; thus, microalgae could serve as a vehicle for IBP uptake by cladocerans, and in consequence, higher toxicity at higher algal density, as more IBP is introduced to the digestive system of chydorids. Xie et al. [43] described a food web in which IBP and other pharmaceutical active compounds were biomagnified.
Fig. 3.
Results of the 5-d test with Lecane papuana exposed to ibuprofen (IBP) and fed on three different algal concentrations of the green alga Nannochloropsis oculata (0.25, 0.50, or 1.00 × 10⁶ cells/mL). All treatments were carried out by quadruplicate. Significant differences (P<0.05) were established through two way ANOVA and multiple comparison tests of Tukey HSD. Statistical analyses were performed with the aid of the package agricolae and graphics were plotted in ggplot2, both in R for Windows.
In contrast, rotifers were exposed to a single load of IBP (at the experiment beginning), and following the ideas described in the previous paragraph, IBP and its metabolites (produced in the first hours of exposure) might have been adsorbed onto microalgae, affected rotifers during the first hours of exposure, and limited their reproduction. However, since there were no further inputs of IB proP, rotifers born from the exposed parental generation could develop in less stressful media, but limited by the food source causing rotifers to produce fewer eggs, and as consequence, reduced their IRPI. Previously, Tovar-Aguilar et al. [22] proved that rotifers born from amictic eggs exposed to diclofenac did not exhibit significant alterations in their reproductive performance in comparison to non-exposed rotifers. Thus, rotifers born in the IBP-contaminated media could develop better because of degradation and removal of IBP and its metabolites, differently to the chydorids, as they were exposed to new inputs of IBP (and its metabolites) every two days. Nevertheless, both hypotheses on cladocerans and rotifers shall be examined in further research as they are beyond the aims of this study: as to describe if IBP is biomagnified from algae to zooplankton; and to study transgenerational effects of IBP on cladocerans and rotifers.
IRPI has been used in ecotoxicology as an indicator of population performance and the effects of environment on such organisms. However, achieving conclusions based on the IRPI has been questioned because of the bias associated with the (over) simplification of calculations [44]. In fact, it is suggested to carry out more complex calculations since computational limitations have been eliminated [45]. However, those authors mentioned that calculation simplifications might be used according to the available data and their goal; thus, we consider that the formulas used in this study contribute to obtaining reliable representations of the population growth rates of the selected zooplankton species, especially when this manuscript does not describe the life cycle of neither of the species, but instead their performance when affected by the combination of two factors: exposure to IBP and food availability (differential algal density).
The environmental concentrations of pharmaceutical active ingredients, like ibuprofen, are generally found within a range of some nanograms per liter in compartments, like freshwater, sea water, or sediments. However, information is mainly available for high-income countries, while in developing countries information is still scarce. Environmental concentration data are relevant to derive the Predicted Non-Effect Concentrations (PNEC), which also depend on the species assayed (in this case, two zooplankters), time of exposure (short or long term exposure), test conditions (i.e., food supplementation, temperature, photoperiod, etc.). Some authors have used different application factors to estimate the PNEC, but such predictions are single-species based. However, Species Sensitivity Distribution (SSD) is an integrative approach that considers several species in the calculation of the Hazard Effect Concentration that affects the 5% (HEC5) of the total populations exposed; thus, results of SSD might better represent the potential effects of chemicals [46].
Trobini et al. [47] estimated the HEC5 for IBP at 4.4 mg/L, which was based on acute toxicity data. As observed, the corresponding LC50 values for either A. guttata or L. papuana are about 15 or 3-fold higher, respectively; therefore, these two species could be considered at no risk, as their LC50 values are much higher than the HEC5. Nevertheless, it is suggested to calculate the PNEC through an application factor (AF) of 5, thus, obtaining the PNEC for IBP at 0.8 mg/L, which might now include data derived from long term toxicity tests or some other endpoints (biomarkers). Then, this PNEC (IBP 0.8 mg/L) is higher than the EC50 (0.524±0.192 mg/L) for L. papuana fed on low algal densities (0.25 × 10⁶ cells/mL), which is the only group (out of the six groups evaluated in this study) not to be protected by that threshold value. However, the highest algal density (1.00 × 10⁶ cells/mL) seems to promote a certain tolerance of L. papuana toward IBP, an effect to be expected as rotifers acquire more energy through algae ingestion and better cope with the intoxication by IBP (Table 3).
Duration of the test (exposure) differed between the two zooplankter species, which was based on their life cycle, with average lifespan of seven days for L. papuana [48], and 60 d for A. guttata [27]. Conventional toxicity tests protocols with rotifers suggest 24 h for acute tests and up to 5 d when assessing alterations on the population increase [16]; for cladocerans the standard protocols include 48-h period for acute toxicity tests and up to 21 d for Daphnia magna in chronic tests [49]. We understand the limitations of the present study and the likely bias due to the different exposure times. Therefore, herein we present some ideas that shall be addressed in further experiments, which are beyond the aim of this study. The generation time (G) in Lecane papuana is about 3-4 days; thus, in the 14-d period (as with A. guttata) we would expect finding not only one rotifers generation but some others, which could be less sensitive to IBP after adaptation, a phenomenon observed in multigenerational and transgenerational toxicity tests [50], then, the rotifers rate of population increase might exhibit higher EC50 values (lower sensitivity), although not at the same level than A. guttata (less sensitive to IBP). Such speculation is based on the results of non-exposed organisms, because exposure to IBP increased the G and reduced the IRPI (Fig. 1). Then, the question of how exposure time interacts with the factors herein studied shall be studied in further experiments, either in single or multi-species protocols. Furthermore, it would be relevant to include the evaluation of algal density throughout the entire test duration. Thereafter, at every sampling time we could obtain information on the density of algae, chydorids, and rotifers. Finally, these sorts of experiments could contribute to a better understanding of the IBP effects on aquatic biota.
Conclusion
IBP significantly altered demographic responses of the zooplankters A. guttata and L. papuana at concentrations below those reported for other species, either the chydorid, which represents a sensitive alternative to D. magna, or L. papuana that is a good alternative to B. calyciflorus. Despite the two zooplankters used in this study presenting similar EC50 values, differences between these two species were observed. Alona guttata seemed not to be affected by the algal density (0.25 to 1.00 × 10⁶ cells/mL), as did L. papuana, which presented the higher sensitivity when fed on the lowest algal density. Thus, the interaction of algal density and IBP at all concentrations negatively affected the population growth of this rotifer, while IBP concentration was the main factor to reduce fertility, survival, and as consequence, the IRPI of A. guttata. Further studies might be required to identify the mechanisms involved in the toxicity of IBP and its metabolites toward zooplankters, as well as IBP biomagnification potential since it was reported to biomagnify under certain conditions.

