

Introduction
Straw resources are huge, though their usage is poor. In October 2024, the latest forecast of the Food and Agriculture Organization of the United Nations for the global output of cereals was 2.853 billion tons [1]. This means that a large amount of crop straw will be produced in the future. China, one of the world's largest producers of crop straw, generates approximately 700 million tons annually [2]. However, more than 10% of straw is still not properly treated, with the majority being burned in the open or discarded randomly [3, 4]. In this scenario, a substantial amount of pollutants further exacerbates issues such as resource wastage and adverse environmental impacts [5, 6]. Consequently, the reuse of straw resources has attracted growing attention [7, 8]. The natural degradation speed of straw is slow due to multiple factors that affect the growth of the next crop. Within them, the characteristics of straw are the basic ones. Straw is mainly composed of cellulose, hemicellulose, and lignin [9]. Lignin is wrapped in cellulose and hemicellulose, whose accessibility requires the elimination of lignin, but the slow degradation of lignin itself limits the degradation of cellulose and hemicellulose, and ultimately limits the natural degradation of straw [10, 11]. There are various ways to accelerate the degradation of straw, among which using straw-degrading bacteria is the most economical and effective way, and seeking the straw-degrading bacteria has become a crucial step [12].
In the context of global climate change, the utilization of microorganisms has become a hot topic [13]. Microbial degradation, as a sustainable straw treatment method, can effectively reduce harmful emissions, promote the recycling of organic matter, and not only alleviate environmental burdens but also convert straw into valuable resources, which is of significant importance to agriculture and ecosystems [14]. Numerous straw-degrading bacteria have been identified. For example, a strain of Aspergillus niger (Aspergillus niger MK543209) was screened in a basic mineral salt medium containing 1% cellulose [15]. The study screened microbial communities that degrade corn straw from straw-degrading bacterial communities, sheep manure, and their mixtures with cow manure. The bacterial communities screened from the three treatments all contained Alternaria alternata [16]. Moreover, a Penicillium strain (Penicillium janthinellum NCIM 1366) was screened by fermentation on Mandels and Weber medium with 1% cellulose as a carbon source [17]. Later, a pure cellulose-degrading bacterium was isolated from sugarcane field soil near a sugar factory in the Indian state of Trengana, and identified through molecular biology as γ-Pseudomonas (Psuedomonas of phylum Gamma-proteobacteria) [18]. Trichoderma viride, identified in the soil of a municipal solid waste dump in Bhopal, Madhya Pradesh, India, can effectively degrade cellulose [19]. It can be seen that different soils screen different specific and efficient bacterial strains. This is because the dominant bacterial species are distinct in different soils, and they recognize and constrain each other. Therefore, selecting the strains or microbial communities for a specific soil can maximize the degradation effectiveness of microorganisms.
The establishment of optimal cultivation conditions for the candidate strains is the basis for industrial production of straw-degrading bacteria. Obviously, the optimal growth conditions for cellulose-degrading bacteria are different. For example, Aspergillus niger MK543209 has an optimal growth temperature of 45℃ and an optimal pH of 5.5 [15] and the optimal fermentation temperature for Trichoderma afroharzianum is 28.8℃, and the optimal pH is 6.32 [19]. Different from them, the optimal growth temperature of Penicillium janthinellum NCIM 1366 is 30℃, and the optimal pH is 4.8 [17]. Moreover, Pseudomonas of phylum Gamma-proteobacteria need a 37℃ and pH 7.0 situation [18], and Hypocrea sp. W63 needs 50℃ and pH 4.8 conditions [20]. It can be seen that after identifying the type of bacterial strain, the optimal growth conditions should also be evaluated based on its specific characteristics to provide a basis for the industrial production of bacterial strains.
The current investigation has shown that inoculating different cellulose-degrading bacteria can improve degradation efficiency under specific conditions. However, few studies have integrated the screening of highly effective cellulose-degrading strains with an analysis of their degradation mechanisms. Therefore, this study utilized straw-return soil as the bacterial source, screened a batch of degrading bacteria, and selected a strain with superior cellulase activity by assessing filter paper enzyme, carboxymethyl cellulase, and microcrystalline cellulase activities. Molecular biological identification was performed to clarify the strain. Furthermore, the metabolic pathways of cellulose-degrading bacteria were concluded, providing candidate strains and a theoretical foundation for the development of high-quality degrading microbial agents to alleviate the problem of straw returning challenges.
Materials and Methods
Sample Collection
The fresh soil samples were taken from the 0-10 cm layer of a farmland in Daqing City, Heilongjiang Province, China, and the five-point sample method was used. The samples were immediately stored at 4℃.
Medium and Configuration
(1) Cultivation medium: sodium carboxymethyl cellulose plate and inclined medium, refer to Chacha’s medium. Sodium carboxymethyl fibroin 5 g, K2HPO4 1 g, AGAR 17 g, NaNO3 3 g, KCl 0.5 g, MgSO4 0.5 g, distilled water 1000 mL, FeSO4 0.01 g, adjust the pH to 5.5-6.0.
(2) Solid PDA medium: peeled potato 200 g, glucose 20 g, MgSO4 2 g, KH2PO4 3 g, peptone 3 g, AGAR powder 20 g, distilled water 1000 mL (all media were sterilized at 121℃ and 0.11 Mpa for 30 min for use).
Enrichment Culture and Screening of Cellulose-Degrading Bacteria
0.1 g of soil sample was weighed and placed in a 100 mL triangular flask with 50 mL of distilled water and some glass beads. After complete dispersion, the mixture was put into a 120 r/min shaking bed and cultivated for 3 days. The enriched solution was diluted to prepare the concentrations of 10, 10-1, 10-2, 10-3, 10-4, and 10-5, respectively. Four replicates for each gradient were detected and separated on the selected medium. After 5 days, the colonies were inoculated into the selected medium. Finally, a total of 63 strains of bacteria were grown normally.
Preliminary Screening of Cellulose-Degrading Bacteria
After vigorous growth, 1 % Congo red solution was used as a coloring agent for 1 h, and NaCl solution was used as a decolorizing agent for 1 h. The cellulose-degrading bacteria with larger hydrolytic circles were retained and regarded as the more highly ability-degraded bacteria. The strains were then selected, crossed, purified, and cultured repeatedly to find the pure strains.
Re-Screening of Cellulose-Degrading Bacteria
The single colony obtained by re-screening was added to the seed medium and shaken at 25℃ and 180 r/min for 72 h, then the obtained fermentation liquid was centrifuged at 4℃ and 6000 r/min for 10 min. The supernatant was regarded as the crude enzyme liquid, which was used for the determination of enzyme activity [17].
(1) Determination of enzyme activity in filter paper
The dinitrosalicylic acid (DNS) colorimetry was used to screen the cellulose strain with high cellulase activity [21]. The prepared crude enzyme solution was added to the filter paper substrate solution, and the mixture was incubated in a 50℃ thermostatic water bath for 1 h. Then, 3 mL DNS solution was added, and the mixed liquid was boiled in a bath full of boiling water for 10 min and immediately terminated with cold water. The control without DNS was the same as the solutions. The optical absorption value (OD value) was measured with a visible spectrophotometer (Shanghai Jingke 723N) at 540 nm. The activity of the filter paper enzyme was calculated according to the glucose standard curve. All the treatments had three replacements.
(2) CMC enzyme activity determination
The prepared crude enzyme solution was added to the CMC substrate solution and incubated in a constant temperature water bath at 50℃ for 30 min. The remaining operation was the same as that of the filter paper enzyme. And the solutions’ OD value is determined under the same conditions.
(3) Determination of microcrystalline cellulose activity
The prepared crude enzyme solution was added to the fine cellulose substrate solution. The reaction was carried out in a constant temperature water bath at 50℃ for 2 h. The remaining operation is the same as the method of filter paper enzyme. The OD value is determined.
Molecular Biological Identification
The first stage was the extraction of strain DNA. The genomic DNA of the strains was extracted according to the operation steps of the bacterial genome extraction kit or fungal genome extraction kit, respectively. NanoDrop2000 was used to detect concentration (μg/ mL) and purity (A260/A280) of extracted DNA, and 1.0 % agarose gel electrophoresis was used to detect DNA integrity.
The second step was PCR amplification and sequencing. Two general primers (Table 1) were used for PCR amplification for the ITS sequence amplification of ribosomal DNA. The reaction system was as follows: 10×TaqDNA polymerase buffer 2.5 μl, dNTP 2.5 μl, TaqDNA polymerase 0.5 μl, PrimerITS4 1 μl, PrimerITS5 1 μl, template DNA 1 μl, ddH2O 16.5 μl. The PCR amplification procedure was as follows: pre-denaturation at 94℃ for 5 min, initial cycle 94℃ 30 s, 52℃ 60 s, 72℃ 45 s, 30 cycles, 72℃ extension for 10 min. The PCR products were identified by 1 % agarose gel electrophoresis. 16SrDNA sequencing. The remaining PCR biochemical reagents were sequenced through commercial services provided by Sangon Bioengineering (Shanghai) Co., LTD. The sequence was then compared with the Ribosomal Database, and the Basic Local Alignment Search Tool (BLAST) program of NCBI was used for homology analysis. A phylogenetic tree was built using the neighbor-joining model of the MEGA4 program.
Experiments on Strain Characteristics
The experiments detected the suitable conditions for cellulose-degrading bacteria by measuring the growth curve at different pH values, temperatures, and different external carbon source concentration conditions.
(1) Configuration of bacterial suspension:The chosen bacteria grew in the PDA medium enriched culture and were diluted to concentrations of 10-2, 10-3, 10-4, 10-5, 10-6, and were coated in the PDA medium for culture. The medium for observation was selected and stored at 4℃.
(2) Study on growth characteristics: Under sterile conditions, 2 mL bacterial suspension was injected into the PDA liquid medium and was shaken at 120 r/min in a constant temperature in a shaking bed for cultures. Then, the strain dry weight was measured each day to detect the growth of the strains, and the growth curve was drawn based on it. The same procedure was used for growth detection, with the only difference being temperature or pH value. 2 mL bacterial suspension was added to the PDA liquid medium and cultured under the conditions of 5℃-30℃ and pH 2.0-13.0, respectively. After the enriched growth of the cultured strains, the dry weight of the strains was measured to detect the optimal growth temperature and pH value. The selective medium was used to detect the effects of substrate concentration on the growth of bacteria by changing the concentration of sodium carboxymethyl cellulose in the medium. With the only factor changed, 2 mL bacterial suspensions with concentrations of 0.05%, 0.15%, 0.25%, 0.35%, 0.45%, and 0.55% were added into PDA liquid medium under different carbon source concentrations. The dry weight of strains was measured to detect the optimal concentration of the carbon source. Three individual replications were used in the experiment.
Results
Screening of Cellulose-Degrading Bacteria
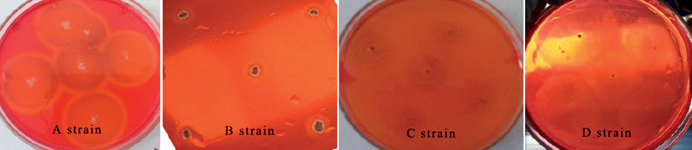
After enrichment and cultivation of the soil samples, we isolated individual colonies using streak plate and dilution plating methods, and initially obtained 63 strains of straw-degrading bacteria through the purification culture of these single colonies. The selected strains were dyed with Congo red for 1 h and then washed with 1 mol/L sodium chloride solution for 1 h. The hydrolysis circles were found with different sizes (as shown in Fig. 1) to identify preliminarily the ability of the strains and labeled as A strain, B strain, C strain, and D strain.
Differences in Enzyme Activity of Cellulose-Degrading Bacteria
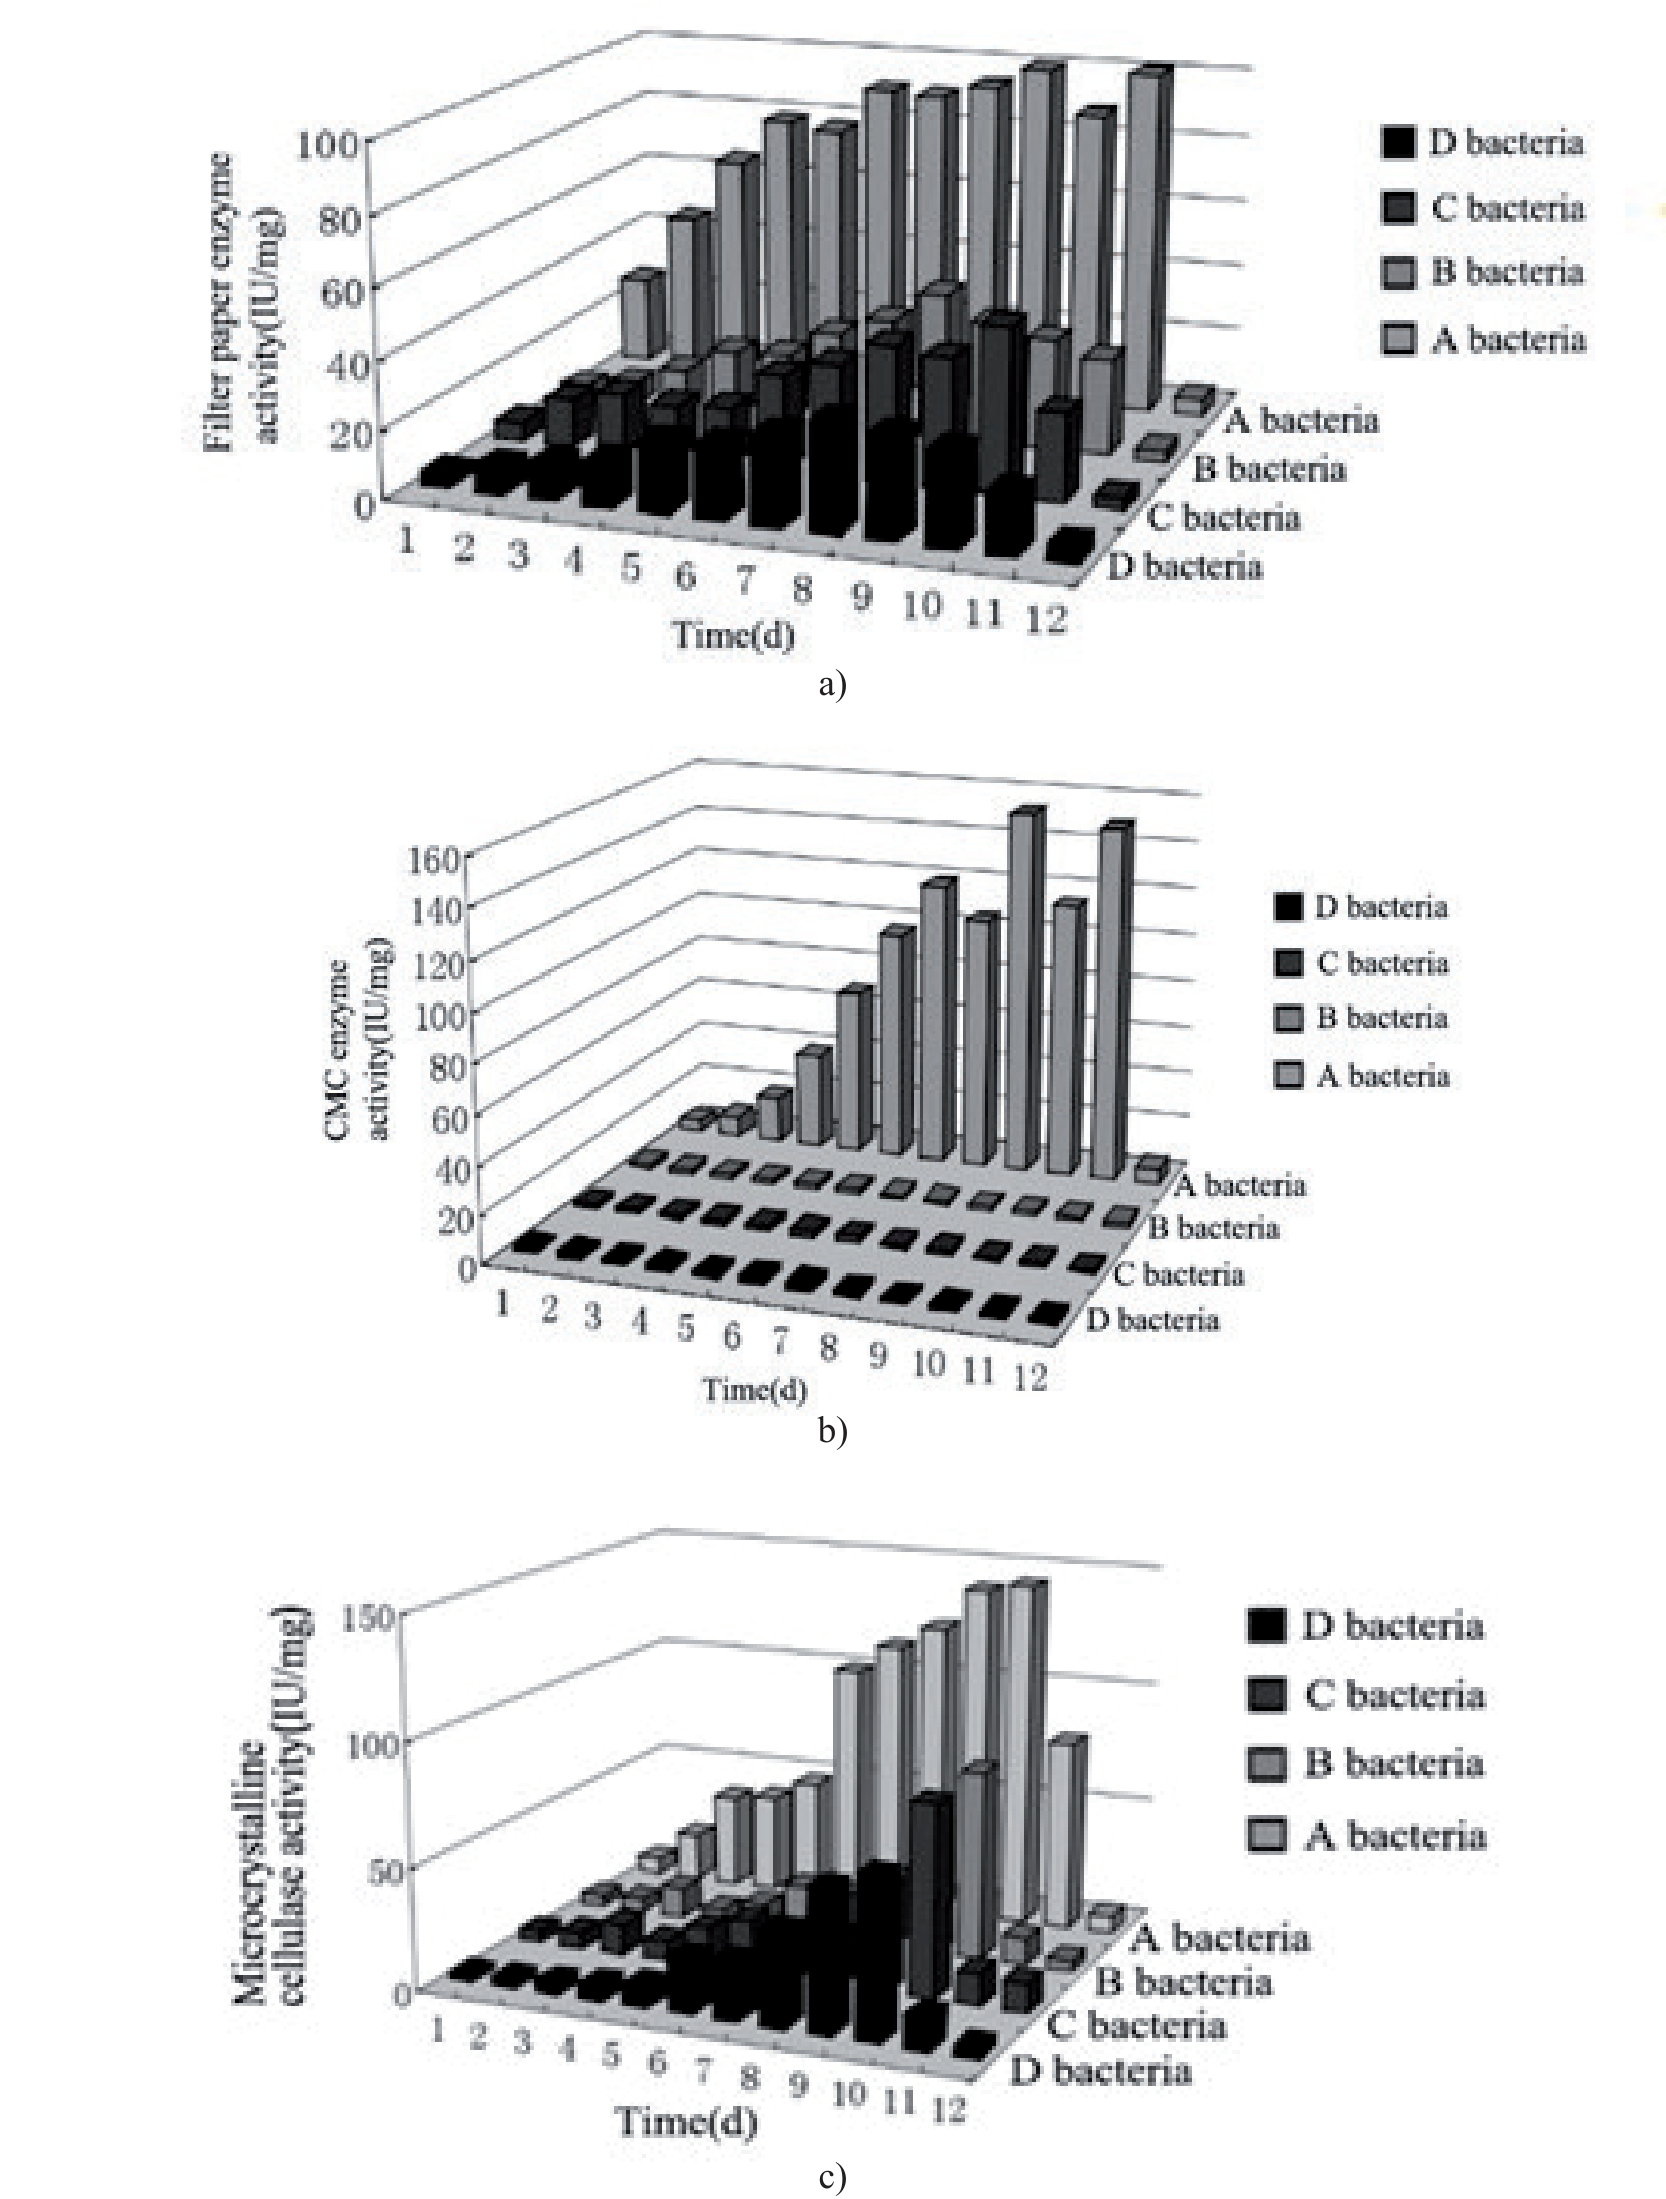
The enzyme activity results of filter paper enzyme, carboxymethyl cellulase, and microcrystalline cellulase were showed in Table 1 and the differences between the enzyme activities of the strains was showed in Fig. 2. The order of filter paper enzyme activity from high to low was A>C>B>D, within them, A had the highest activity of filter paper enzyme, 102.13 IU/mg. The order of carboxymethyl cellulase activity from high to low was A>B>D>C. The carboxymethyl cellulase activity values of B and D were at the same level, and A had the highest carboxymethyl cellulase activity, designated as 153.45 IU/mg. The order of activity of microcrystalline cellulase from high to low was A>D>C>B. Among them, A has the highest activity of microcrystalline cellulase, which was 144.22 IU/mg.
Molecular Biological Identification
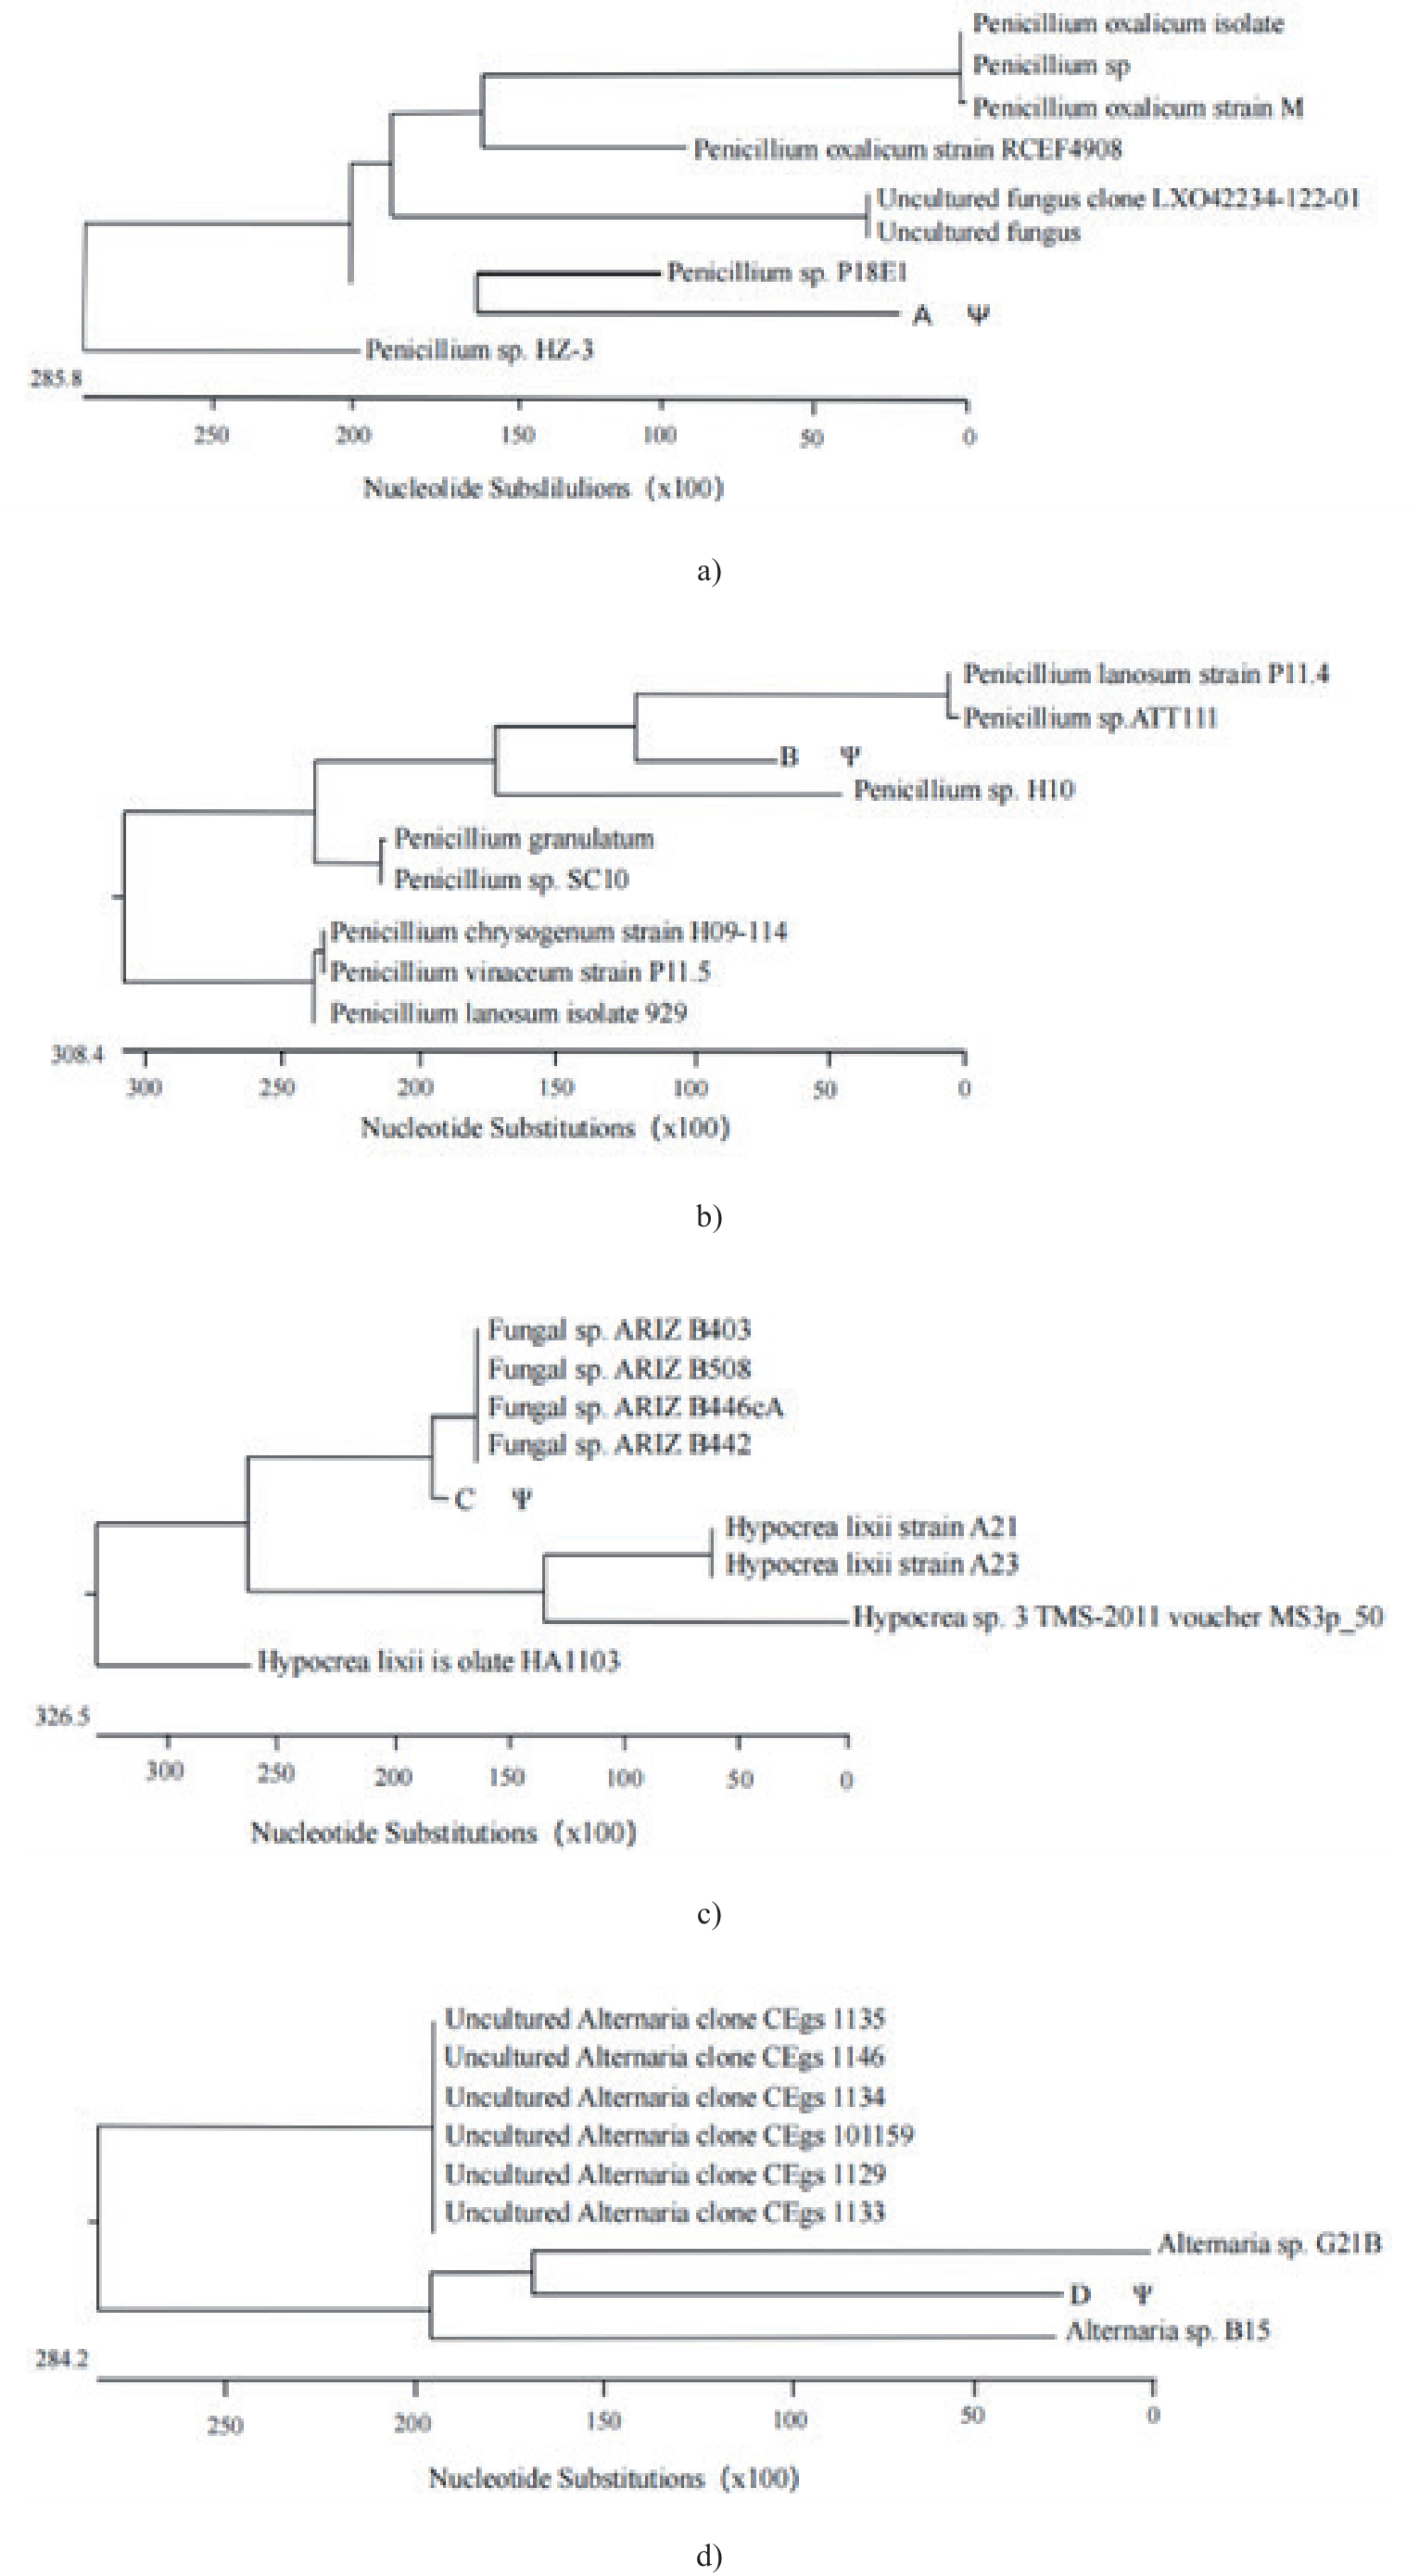
The ITS sequence lengths of strains A, B, C, and D were detected as 578 bp, 612 bp, 636 bp, and 574 bp, respectively (Fig. 3). After BLAST alignment on NCBI, the highly homologous sequences belonged to the gene sequences of the genus Actinobacteria, a kind of fungi, with a homology of over 99%. The gene sequence of A shares 99% homology with Penicillium sp.; Similarly, the 99% homology was found in the gene sequence of B and the gene sequence of Penicillium vinaceum strain P11.5, the gene sequence of C and Hypocrea sp. Moreover, the gene sequence of D had 100% homology with Alternaria sp. The ITS sequence homology of the strains was analyzed, and the results identified that A was Penicillium vinaceum, and B was Hypocrea sp. Meanwhile, C was regarded as Phenerochaetic chrysosporium and D was regarded as Alternaria.
Research on the Characteristics of Bacteria
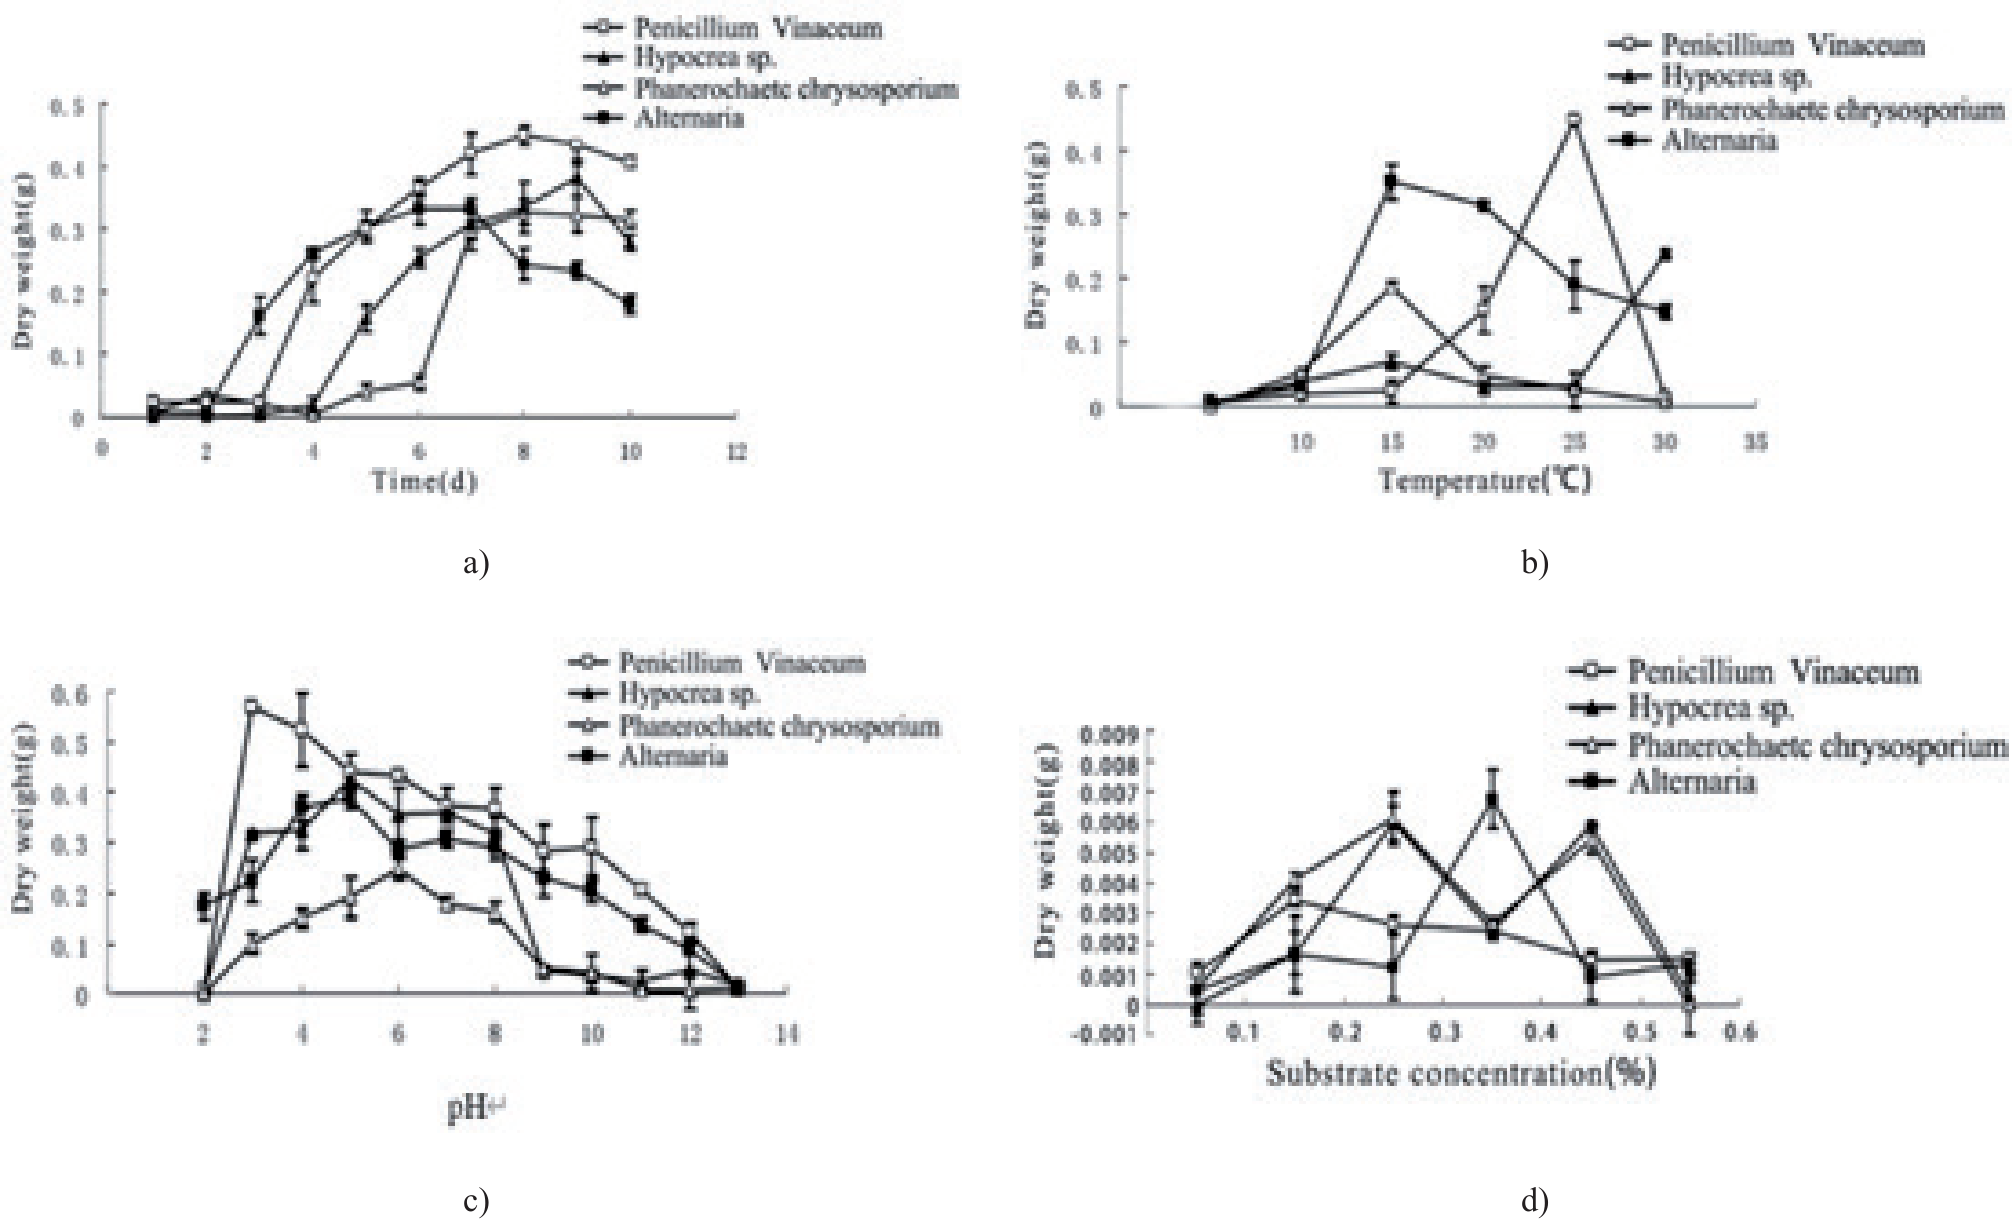
Four selected cellulose-degrading bacteria had different optimal growth conditions (Fig. 4). Penicillium Vinaceum (A), Hypocrea sp.(B), Phanerochaetic Chrysosporium (C), and Alternaria (D) had the highest biomass at the 8th, 9th, 6th to 8th, and 6th day of cultivation, respectively, indicating that the optimal growth conditions for the bacterial species occurred within the cultivation period. By deep analysis, the optimal temperature was found to differ in the candidate strains. That of Penicillium Vinaceum and Hypocea sp. was at 25℃ and 30℃, relatively higher among the strains, with the dry weights of 0.448 g and 0.240 g. The optimal growth temperature for Phanerochaetic chrysosporium and Alternaria was 15℃ with the dry weights of 0.188 g and 0.351 g, respectively. Meanwhile, the candidate strains grow better under the acidic conditions, with the optimal pH value being 5.0 for Hypocrea sp. and Alternaria, with the dry weights of 0.424 g and 0.387 g, respectively. The optimal pH values for Penicillium vinaceum and Phanerochaetic chrysosporium were 3.0 and 6.0, with the dry weights of 0.567 g and 0.249 g, respectively. The optimal substrate concentrations for the four candidate strains were different. The one for the strain Penicillium vinaceum was 3 g/L (dry weight 0.0035 g), whereas the one for the strains Hypocrea sp. and Phanerochaetic chrysosporium was 5 g/L (dry weight 0.006 g). The one for strain Alternaria was 7 g/L (dry weight 0.007 g).
Fig. 3.
Phylogenetic tree results. a) A bacterial phylogenetic tree, b) B bacterial phylogenetic tree, c) C bacterial phylogenetic tree, d) D bacterial phylogenetic tree.
Discussion
The straw-degrading soil was used to screen efficient straw-degrading bacteria, and four strains with strong degradation ability were obtained. There are studies indicating that setting special screening conditions can screen out strains with desired functionalities, thereby more effectively addressing the research objectives [14, 22]. Moreover, the strain A was confirmed as Penicillium vinaceum, a species of Penicillium, with the strongest degradation ability among the selected strains. The best growth conditions, including temperature of 25℃, pH 3.0, and substrate concentration of 3 g/L, were optimal for the strain A. Contrary to the findings, the optimum growth temperature of Penicillium janthinellum NCIM 1366 was 30℃, and the optimum pH was 4.8 [17]. Compared to Penicillium vinaceum, it can tolerate lower pH values and temperatures; its optimal growth temperature is 25℃. Penicillium chineulatum 2HH grew vigorously at 96 h of cultivation, with cellulose as the carbon source, an initial pH of 4.8, and a temperature of 50℃. At this time, the mycelium grows approximately 5.7 g/L. Under the same culture conditions, the growth of Penicillium chineulatum S1M29 was at the most vigorous level at 48 h, with mycelium growth of about 5.4 g/L [23]. A strain of Penicillium sp. FSDE15 was selected from soil samples from the sugarcane plantation in Paraiba Santa Rita, Brazil. Under sterile conditions at 37℃ and pH 5.7, the maximum carboxymethyl cellulase activity value was observed to be 1.38 U/mL within 120 h using sugarcane bagasse as the culture medium [24]. It can be seen that the difference in the growth environments results in different adaptations of Penicillium. The strong degradation ability of Penicillium on straw is due to the synergistic effect of its highly active extracellular multi-enzyme system [25, 26]. It has been discovered that Penicillium produces a highly active exoglycanase, β-glucosidase, with an activity 3.7 times greater than Trichoderma [27]. They provided efficient nutrients for the biomass saccharification process, thereby reducing the demand for cellulase and reducing the cost of cellulase in the production process [28, 29].
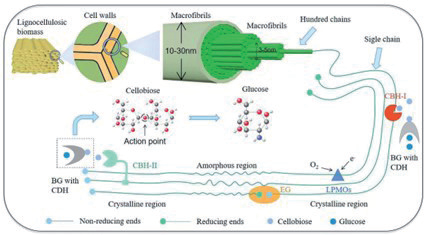
The cellulase produced by Penicillium has a finely coordinated process to achieve the degradation of plant polymers, and the mechanism of action of cellulase is substrate-specific [30]. For example, endocellulases (EGs) act on the amorphous region of cellulose and destroy it from its internal structure β-1,4-neneneba glycosidic bond, exposing the reducing terminal and non-reducing terminal to start hydrolysis; Extracellular cellulase (CBH) has two isomers, CBH-I and CBH-II, which break from the terminal of the chain β-1,4- neneneba glycosidic bond and release cellobiose or cellobiose. And β-Glucosidase (BGs) acts on the non-reducing terminal of cellulose oligosaccharide or cellulose disaccharide to hydrolyze it into glucose. The effects of EGs, CBH, and BGs on cellulose can be summarized as the mechanism of cellulase to completely hydrolyze cellulose into glucose [31, 32]. In addition, lysolysaccharide monooxygenases (LPMOs), as auxiliary active enzymes, are also powerful tools for degrading cellulose raw materials [33, 34]. Gerdt Müller et al. found that LPMOs split the glycosidic bond of crystalline cellulose through the hydroxylation of the C1 or C4 position of the sugar ring, creating an entrance for other cellulase hydrolyses to digest biomass further, thus improving the conversion efficiency [35-37].
Based on the above analysis, we believe that the degradation mechanism of cellulose under the action of Penicillium bicolor is achieved through the dissolution of CBH-I and LPMOs, as well as the separation of CBH-II and EGs. The degradation process involves multiple mechanical steps [38]. Firstly, the movement of enzymes to the substrate surface is through a diffusion system. Secondly, through the pore structure, enzymes are further transferred to the substrate particles and adsorbed onto the adsorbent sites, leading to enzymatic hydrolysis reactions on the cellulose surface (Fig. 5) [39]. In the presence of LPMOs, various cellulases have a synergistic effect on the degradation of cellulose chains. In the reaction, CBH-I and CBH-II reduce the reducing and non-reducing terminals, respectively. EGs randomly attack the glycosidic bond in the amorphous region of the cellulose chain, increasing the number of free ends, which are further degraded by cellulose hydrolase. LPMOs cleave the chains in the crystal region by consuming O2 and e-, while BGs collaborate with cellobiose dehydrogenase (CDHs) to cleave cellobiose into glucose [40]. It is precisely due to the action of the extracellular multi-enzyme systems that they have a high ability to degrade cellulose.
The Penicillium vinaceum screened in this study showed excellent performance in cellulose degradation ability (Fig. 2), with filter paper enzyme, carboxymethyl cellulase, and microcrystalline cellulase activities reaching 102.13 IU/mg, 153.45 IU/mg, and 144.22 IU/ mg, respectively, compared to the highest carboxymethyl cellulase activity of Aspergillus niger MK543209, 4.36 U/mL [15], and the highest filter paper enzyme activity of Trichoderma afroharzianum 0.91 U/mL [19]. The highest filter paper enzyme activity of Penicillium janthinellum NCIM 1366 was 6.59 U/mL [17]. The carboxymethyl cellulase activity of Pseudomonas of phylum Gamma-proteobacteria was 1.2 U/mL [18]. By comparison, it was found that Penicillium vinaceum not only demonstrates heightened activity in three enzyme activities, but also exhibits tolerance to low temperatures and acidity (optimal at 25℃ and pH 3.0). This feature indicates a significant competitive advantage in the development of efficient straw-degrading microbial agents, providing an effective candidate strain resource for solving the obstacle of straw returning to the field.
Conclusions
Four high-efficiency cellulose-degrading bacteria were obtained, namely Penicillium vinaceum, Hypocrea sp., Phanerochaetc chrysosporium, and Alternaria. Within them, Penicillium vinaceum had the best straw degradation ability. Its filter paper enzyme activity, endoglucanase activity, and exoglucanase activity are 102.13 IU/mg, 153.45 IU/mg, and 144.22 IU/mg, respectively. The optimal growth temperature for Penicillium vinaceum is 25℃, the pH value is 3.0, and the substrate concentration is 3 g/L. Analysis of the degradation ability of Penicillium bicolor revealed that its mechanism lies in the dissolution of CBHI and LPMOs, as well as the separation of CBH-II and EGs, which together decompose cellulose into cellobiose, while BGs and CDHs synergistically cleave cellobiose into glucose.
The low-temperature acid resistance of Penicillium vinaceum allows it to directly adapt to the environment of straw decomposition in the field, which can save the cost of temperature and pH control in the application of traditional microbial agents. Future research can be developed from the following three aspects: (1) Develop a composite microbial agent based on Penicillium vinaceum and construct a synergistic degradation system by combining efficient cellulose degrading strains screened from other studies; (2) Enhance the expression stability of key enzymes, such as LPMOs and CDHs, using gene editing technology; (3) Establish the "bacteria enzyme co-production" process to simultaneously produce cellulose degrading bacterial agents and related cellulase preparations.
The application of Penicillium vinaceum can promote the transition of straw returning from physical property fragmentation to biologically efficient decomposition, providing microbial technology support for solving the obstacle problem of straw returning, and providing ideas for developing lower-cost cellulose degradation.

