Introduction
Composting, recognized as an economical and effective organic waste treatment method, garners considerable attention for its reliance on microbial and enzymatic actions to decompose unstable solid organic matter into stable humus [1, 2]. Presently, composting techniques are categorized into two groups: natural composting and artificial composting [3, 4]. Among them, natural composting is the more traditional and common method, which makes use of the decomposition of microorganisms in nature to convert organic wastes into organic fertilizers [5]. However, the natural composting process necessitates an extended fermentation period. Cow dung as a composting raw material [6] not only supplies a substantial quantity of nutrients and organic matter for composting [7, 8] but also enhances plant productivity [9]. Simultaneously, it efficiently mitigates emissions of GHGs, NH3, VOCs, and other gas emissions [10, 11]. Straw as an auxiliary feedstock for composting can not only provide a source of compost organic matter carbon for composting, regulate the C/N ratio, enhance compost porosity [12], and regulate the structure of microbial communities [13], but also contribute to the reduction of environmental pollutants like CH4 and N2O [14], and increase the added value of agricultural waste in economic, environmental, or social terms [15]. The annual production of straw in China is about 7.06×10⁸ t, and that of livestock manure is about 2×10⁹ t [16]. Both straw and livestock manure contain a large amount of cellulose, hemicellulose, and lignin, representing abundant biomass resources in nature [17]. Cellulase can be used for the development of this biomass resource. Cellulase is a general term for a group of enzymes that can degrade cellulose into simple sugars, rather than referring to one enzyme alone. It primarily comprises endoglucanase, exoglucanase, and β-glucosidase. Cellulose-degrading bacteria can synthesize these enzymes and utilize them for cellulose degradation. However, the close arrangement of atoms in cellulose crystals renders it impermeable to enzymes and water molecules [18]. At the same time, the lignin in the plant cell wall is connected with cellulose, relying on hydrogen bonding, which hinders the contact between cellulose and enzymes, although lignin does not damage the enzymatic reaction of cellulose, which leads to a longer fermentation time in natural composting techniques [19]. Hence, we need more efficient cellulose-degrading bacteria to enhance degradation efficiency.
Composite fungicide generally refers to a system formed by mixing two or more single bacteria. Research has demonstrated that synergy exists among microorganisms during the composting process, with a single strain having a lower role in accelerating cellulose degradation than the combined effect of a composite microflora [20]. Moreover, the composite microflora demonstrated the capability to enhance the diversity of cellulose-degrading genes and communities within the compost [21], stimulate the potential functions and interactions of the flora, and augment the cellulose-degrading bacterial degradation capacity in the original compost [22]. For the current urgent situation, this approach can take full advantage of more efficient microbial degradation systems for cellulose. Utilizing this method is a more appropriate option given the long duration of current natural composting techniques, the difficulty of converting waste into an effective resource, and the urgency for production [19, 22].
In Heilongjiang, China, a major grain-producing province, the ambient temperature is around -16ºC in winter. Low ambient temperatures are a challenge for natural composting because low temperatures result in reduced microbial abundance, simplified composition, and suppressed activity, which in turn leads to decreased composting efficiency [23, 24]. In order to ensure the normal operation of composting, some compost heating methods have been extensively studied, such as natural gas heating, biogas heating [25], electric heating, and solar heating [26, 27]. These heating techniques aim to enhance microbial activity in the compost at low temperatures [23]. However, these methods are costly and energy-intensive, limiting their potential effectiveness in practical composting applications [28, 29]. Previous research indicates that cold-adapted microorganisms have their own adaptive ability to cope with cold stress and can maintain high activity in low-temperature environments [30-32]. Therefore, screening for cold-adapted microorganisms is of high practical value.
In this study, natural compost was used as the bacterial source and cellulose as the only carbon source, and the low-temperature efficient cellulose-degrading bacteria were initially screened, and antagonistic experiments and one-way variable experiments were used to further study the interaction system that exists among the composite strains under low-temperature conditions and to ultimately determine the mixed flora with the best cellulose-degrading effect and its optimal enzyme-producing conditions. These findings provide a theoretical basis and technical support for the optimization of the low-temperature composting process of straw and livestock manure at a later stage, so as to better solve the problems of pollution and resource wastage of the accumulation of straw and livestock manure under low-temperature conditions.
Materials and Methods
Sample Collection and Processing
The samples were taken from a natural compost pile in Xinyi Village, Harbin City, the pile (2.8 m long, 1 m wide, and 0.8 m high), with the main components of which are the mixed fermentation products of straw and animal manure. In the pre-composting period (2 d of fermentation), 2 points were randomly selected from the upper, middle, and lower layers of the compost (10, 30, and 60 cm) for sampling, totaling 6 samples, and the obtained compost fresh samples were packed into pre-inactivated bacteriological sealing bags and then retrieved for use after being wrapped. The six samples were mixed well to obtain the original sample to be tested.
Isolation and Purification of Cellulose-Degrading Bacterial Strains
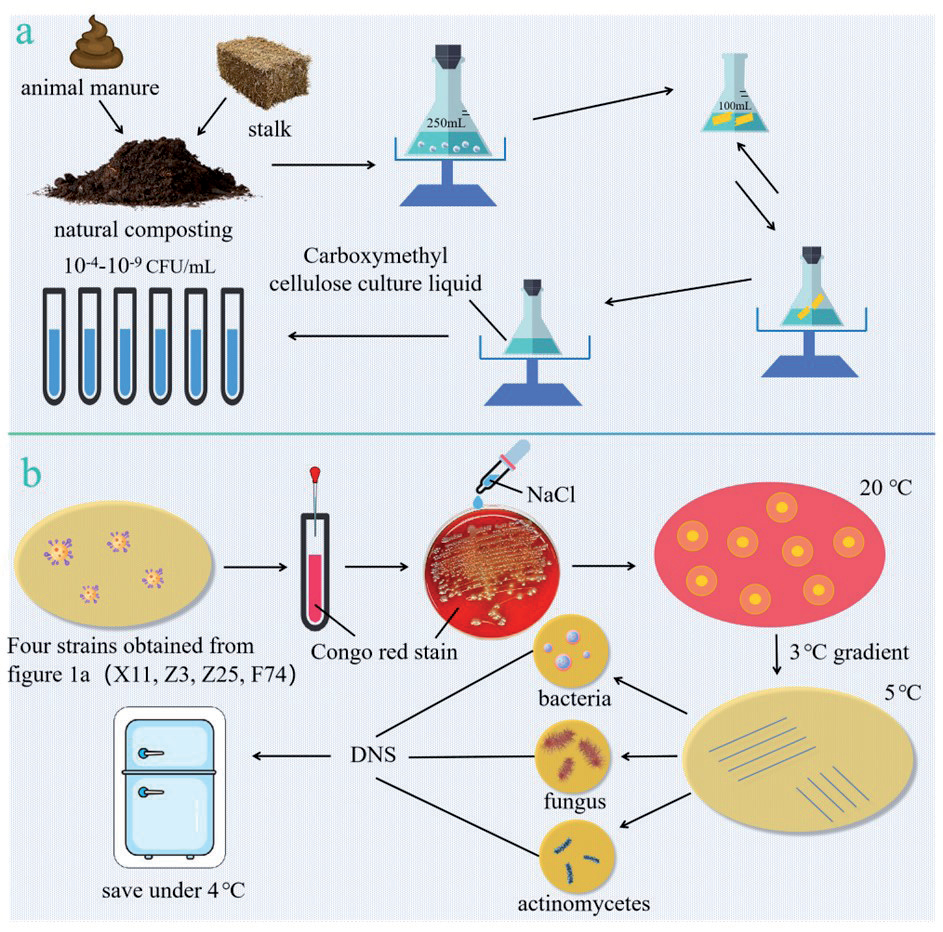
A direct isolation method was employed to obtain strains with the capability to utilize cellulose as the sole carbon source [33]. As shown in Fig. 1a), 10 g of the original sample was placed into a 250 mL triangular flask containing small glass beads, 100 mL of sterilized distilled water was added, and the suspension was shaken at 20ºC for 30 min at 120 r/min, so that the strains were completely free and evenly distributed in the water. Take 1 mL of the suspension and add it to a triangular flask containing 100 mL of Hutchison’s liquid medium and incubate it at 20ºC. After the filter paper disintegrated, the culture was shaken at 20ºC and 120 r/min for 30 min, and then transferred to fresh Hutchison’s liquid medium, the inoculum amount was 10% each time, and so on for several generations, eliminating the cultures that had lost the ability to decompose and were unstable. The culture solution was taken from the culture, and under the condition of aseptic operation, the culture was picked from the broken filter paper strip, transferred to fresh CMC liquid medium, and incubated in constant temperature oscillation at 20ºC and 120 r/min for 2-5 d. Under the condition of aseptic operation, the bacterial stock solution was diluted in accordance with the concentration gradient of 10-4-10-9, and the obtained dilution was spread on the CMC medium plate. Under the condition of aseptic operation, the bacterial stock solution was diluted according to different concentration gradients of 10-4-10-9, and the obtained dilutions were spread on CMC medium plates, and the plates were incubated at 20ºC for 2-5 d to obtain single colonies. The single colonies were repeatedly streaked and purified until a pure strain was obtained.
Fig. 1.
Schematic illustration for the cellulose-degrading bacteria screening process via two steps: a) Isolation and purification of cellulose-degrading strains. b) Screening and conservation of these identified strains.
Hutchison liquid medium: l g KH2PO4, 0.01 g FeCl3, 0.3 g MgSO4-7H2O, 2.5 g NaNO3, 0.1 g CaCl2, 0.1 g NaCl, 1 000 mL H2O, pH 7.0-7.4.
Carboxymethyl cellulose medium: 15 g CMC-Na, 1 g NH4NO3, l g yeast extract, 0.5 g MgSO4-7H2O, l g KH2PO4, 20 g agar, l 000 mL H2O.
Screening and Preservation of Cellulose-Degrading Bacterial Strains
The isolated and purified strains underwent initial screening using the Congo red staining method. As shown in Fig. 1b), the single bacterial spots obtained after isolation and purification were inoculated on CMC medium, and the colonies were grown after 2-5 d of incubation at 20ºC. An appropriate amount of Congo Red staining solution was added to the plate and stained for 1 h. The staining solution was discarded and washed for 1 h with an appropriate amount of NaCl solution. The presence or absence of a hydrolysis circle was used to determine whether it was a cellulose-degrading bacteria. Based on the diameter of the hydrolysis circle, strains demonstrating superior cellulose degradation were initially selected. By regulating the temperature, the strains were screened for their ability to grow even under low temperature conditions. The strains obtained from the initial screening were streaked and cultured on CMC medium for 2-5 d. The temperature gradient of 3ºC was used for cooling, and the growth of the strains and the number of survivors were observed after each cooling to finally obtain the lowest temperature for the growth of the strains. The total enzyme activity, endoglucanase activity, and exoglucanase activity were assessed through the dinitrosalicylic acid (DNS) colorimetric assay. The filter paper degrading enzyme activity was employed to indicate the total enzyme activity, CMC degrading enzyme activity represented the endoglucanase activity, and microcrystalline cellulose enzyme activity denoted the exoglucanase activity [34-37]. Under the condition of aseptic operation, the strain obtained by re-screening was inoculated on the slant medium by using the scribing method, and after growing colonies for 2-5 d at 20ºC, it was placed in the refrigerator at 4ºC for storage. In order to maintain the activity of the strain, it was usually transferred once every 1-2 months.
Molecular Biology Identification
Extraction of strain DNA: DNA is extracted from the organism and subsequently processed through standard molecular biology experimental procedures.
PCR amplification and sequencing: the strains that have been isolated were sequenced with primers 27f: 5’-AGAGTTTGATCCTGGCTCAG-3’ and 1492R: 5’-GGTTACCTTGTTACGACTT-3’ (for bacteria and actinomycetes), NS1: 5’-GTAGTCATATGCTTGTCTC-3’ and NS8: 5’-TCCGCAGGTTCACCTACGGA-3’ (for fungi) [38] and amplified by PCR. The reaction system was: 1 μL of primer 27f (10 μM), 1 μL of primer 1492R (10 μM), 5 μL of 10×EasyTaq Buffer, 4 μL of dNTPs (2.5 mM), 0.5 μL of EasyTaq DNA Polymerase, 1 μL of DNA buffer, and 37.5 μL of sterilized deionized water (for bacterial vs. actinobacteria). Primer NS1 (10 μM) 1 μL, primer NS8 (10 μM) 1 μL, 10×EasyTaq Buffer 5 μL, dNTPs (2.5 mM) 4 μL, EasyTaq DNA Polymerase 0.5 μL, DNA Buffer 1 μL, and sterilized deionized water 37.5 μL (for fungi). The PCR amplification procedure was 94. The PCR amplification program was as follows: pre-denaturation at 94ºC for 10 min, start the cycle, denaturation at 94ºC for 30 s, annealing at 50ºC for 45 s, extension at 72ºC for 100 s, 35 cycles, and stabilization at 72ºC for 10 min (for bacteria and actinomycetes). Pre-denaturation at 94ºC for 5 min, start the cycle, denaturation at 94ºC for 40 s, annealing at 60ºC for 60 s, extension at 72ºC for 90 s, 30 cycles, and stabilization at 72ºC for 10 min (for fungi). The PCR amplified products were sent to UW Genome Technology Co. for sequencing. The measured results were compared with the data on Genbank to find the homologous sequences and analyzed.
Cultivation Studies of Mixed Bacteria and Determination of Enzyme Activity
The antagonism test was carried out on the identified dominant strains. Two different bacteria were drawn parallel lines on the CMC plate medium and incubated at 20ºC for 2-5 d to observe whether there was any antagonism phenomenon. The turbidimetric method was used to investigate the growth of a mixture of bacteria by taking advantage of light impermeability of the bacteria to light. The bacterial solution to be tested was diluted 10-fold, and shaken well, and the culture solution without inoculum was used as a blank control, and the optical density value was determined using a spectrophotometer at a wavelength of 560 nm. The strains without antagonism were mixed, and the enzyme activity was determined in the same way as for single bacteria. The dominant mixed bacteria were screened by determining enzyme vigor.
Optimization of Enzyme Production Conditions for Mixed Bacteria
To investigate the effect of incubation time on cellulase enzyme activity, the screened dominant mixed bacteria were inoculated into the liquid medium, and the CMC degrading enzyme activity was measured every 24 h, and consecutively until the enzyme activity began to decline, to determine the period of maximum enzyme activity as well as the change of the enzyme activity during the whole growth process; to investigate the effect of initial pH on cellulase activity, on the basis of the period of maximum enzyme activity has been determined, set the initial pH range of 3.0-11.0, determine the CMC degrading enzyme activity of the mixed bacteria, and determine the optimal enzyme-producing initial pH; to investigate the effect of incubation temperature on cellulase activity, on the basis of the period of maximum enzyme activity has been determined and the optimal enzyme-producing initial pH, set the incubation temperature. The range was 5-15ºC, and the CMC degrading enzyme activity of the mixed bacteria was determined to determine the optimal enzyme-producing temperature; the effect of inoculum amount on cellulase enzyme activity, based on the period of maximum enzyme activity, the optimal initial pH for enzyme production and the optimal enzyme-producing temperature had been determined, the range of inoculum amount was set from 0.5 to 7%, and the CMC degrading enzyme activity of the mixed bacteria was measured to determine the optimal inoculum amount for enzyme production.
Investigation of Degradation by Mixed Bacteria
The weight loss method was used to determine the degradation rate of the mixed bacteria. The test of degradation of filter paper by cellulose degrading bacteria was carried out by drying the filter paper to a constant weight and adding it to the culture medium, washing and drying the filter paper at the end of the test, recording the constant weight of the filter paper before and after the test, finding the difference in weights, calculating the rate of weight loss, and studying the degradation of cellulose by the mixed bacteria through the rate of weight loss of the filter paper. Under the optimal conditions for enzyme production, the mixed bacteria were inoculated into 100 mL of PPCS medium (containing 0.5 g of filter paper) for static incubation with three replicates. The culture solution underwent centrifugation at 6000 r/min for 5 min, followed by removal and washing of the supernatant. Subsequently, it was centrifuged again at 6000 r/min for 5 min, washed with a hydrochloric acid and nitric acid mixture to eliminate bacterial residues, further washed with water, and centrifuged. The resulting sample was then dried at 105ºC and weighed. The following formula was used to calculate the degradation rate [39]
Results and Discussion
Enzyme Activity Analysis of Low-Temperature Cellulose-Degrading Bacteria
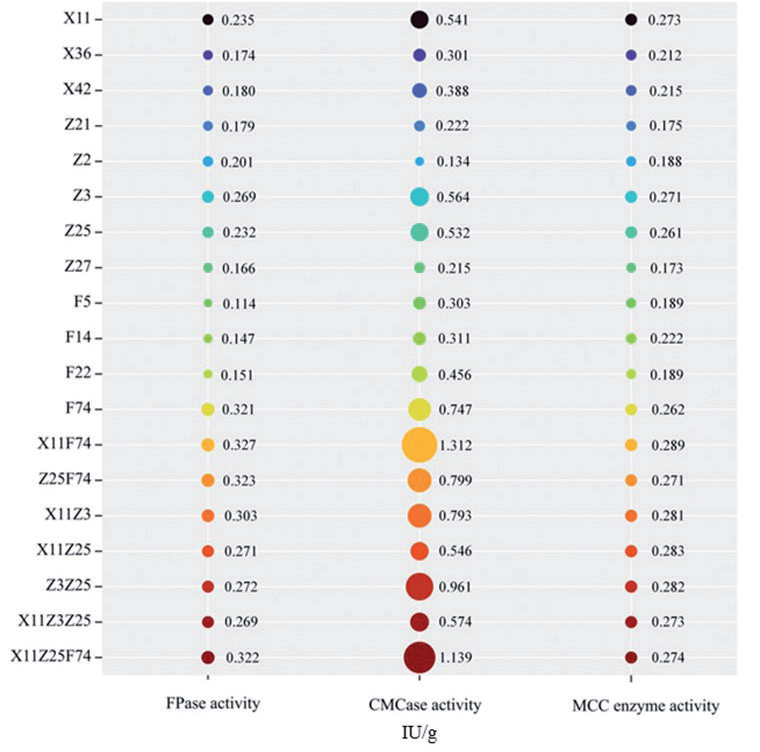
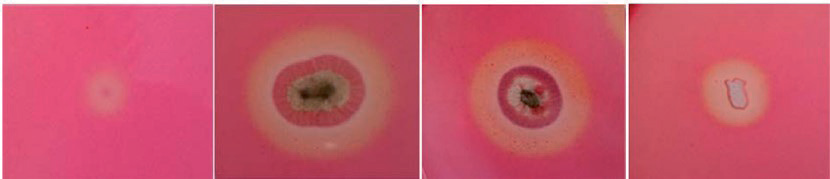
Through isolation, purification, as well as primary and secondary screening, 12 strains of low-temperature cellulose-degrading microorganisms were finally obtained, named X11, X36, X42 (bacteria), Z2, Z3, Z21, Z25, Z27 (fungi), and F5, F14, F22, F74 (actinomycetes). The strains were inoculated into the corresponding liquid media according to class, and the effect of each strain on the enzyme activities of filter paper degrading enzyme, CMC degrading enzyme, and microcrystalline cellulase was different, as presented in Fig. 2. Among the three types of strains, the highest filter paper degrading enzyme activities were found in X11, Z3, and F74, with corresponding enzyme activities of 0.235 IU/g, 0.269 IU/g, and 0.321 IU/g. The highest CMC degrading enzyme activities were found in X11, Z3, and F74, with corresponding enzyme activities of 0.541 IU/g, 0.564 IU/g, and 0.747 IU/g. The highest microcrystalline cellulose enzyme activities were also found in X11, Z3, and F74, with corresponding enzyme activities of 0.273 IU/g, 0.271 IU/g, and 0.262 IU/g. Furthermore, the filter paper degrading enzyme activity of Z25 was 0.232 IU/g, the CMC degrading enzyme activity was 0.532 IU/g, and the microcrystalline cellulose enzyme activity was 0.261 IU/g, which was very similarly different from the three enzyme activities of Z3. Therefore, bacteria X11, fungi Z3 and Z25, and actinomycetes F74 were finally identified as candidate cryogenic strains for cellulose degradation. The four cellulose-degrading bacteria obtained by Congo red staining are shown in Fig. 3.
Molecular Biology Identification of Low-Temperature Cellulose-Degrading Bacteria
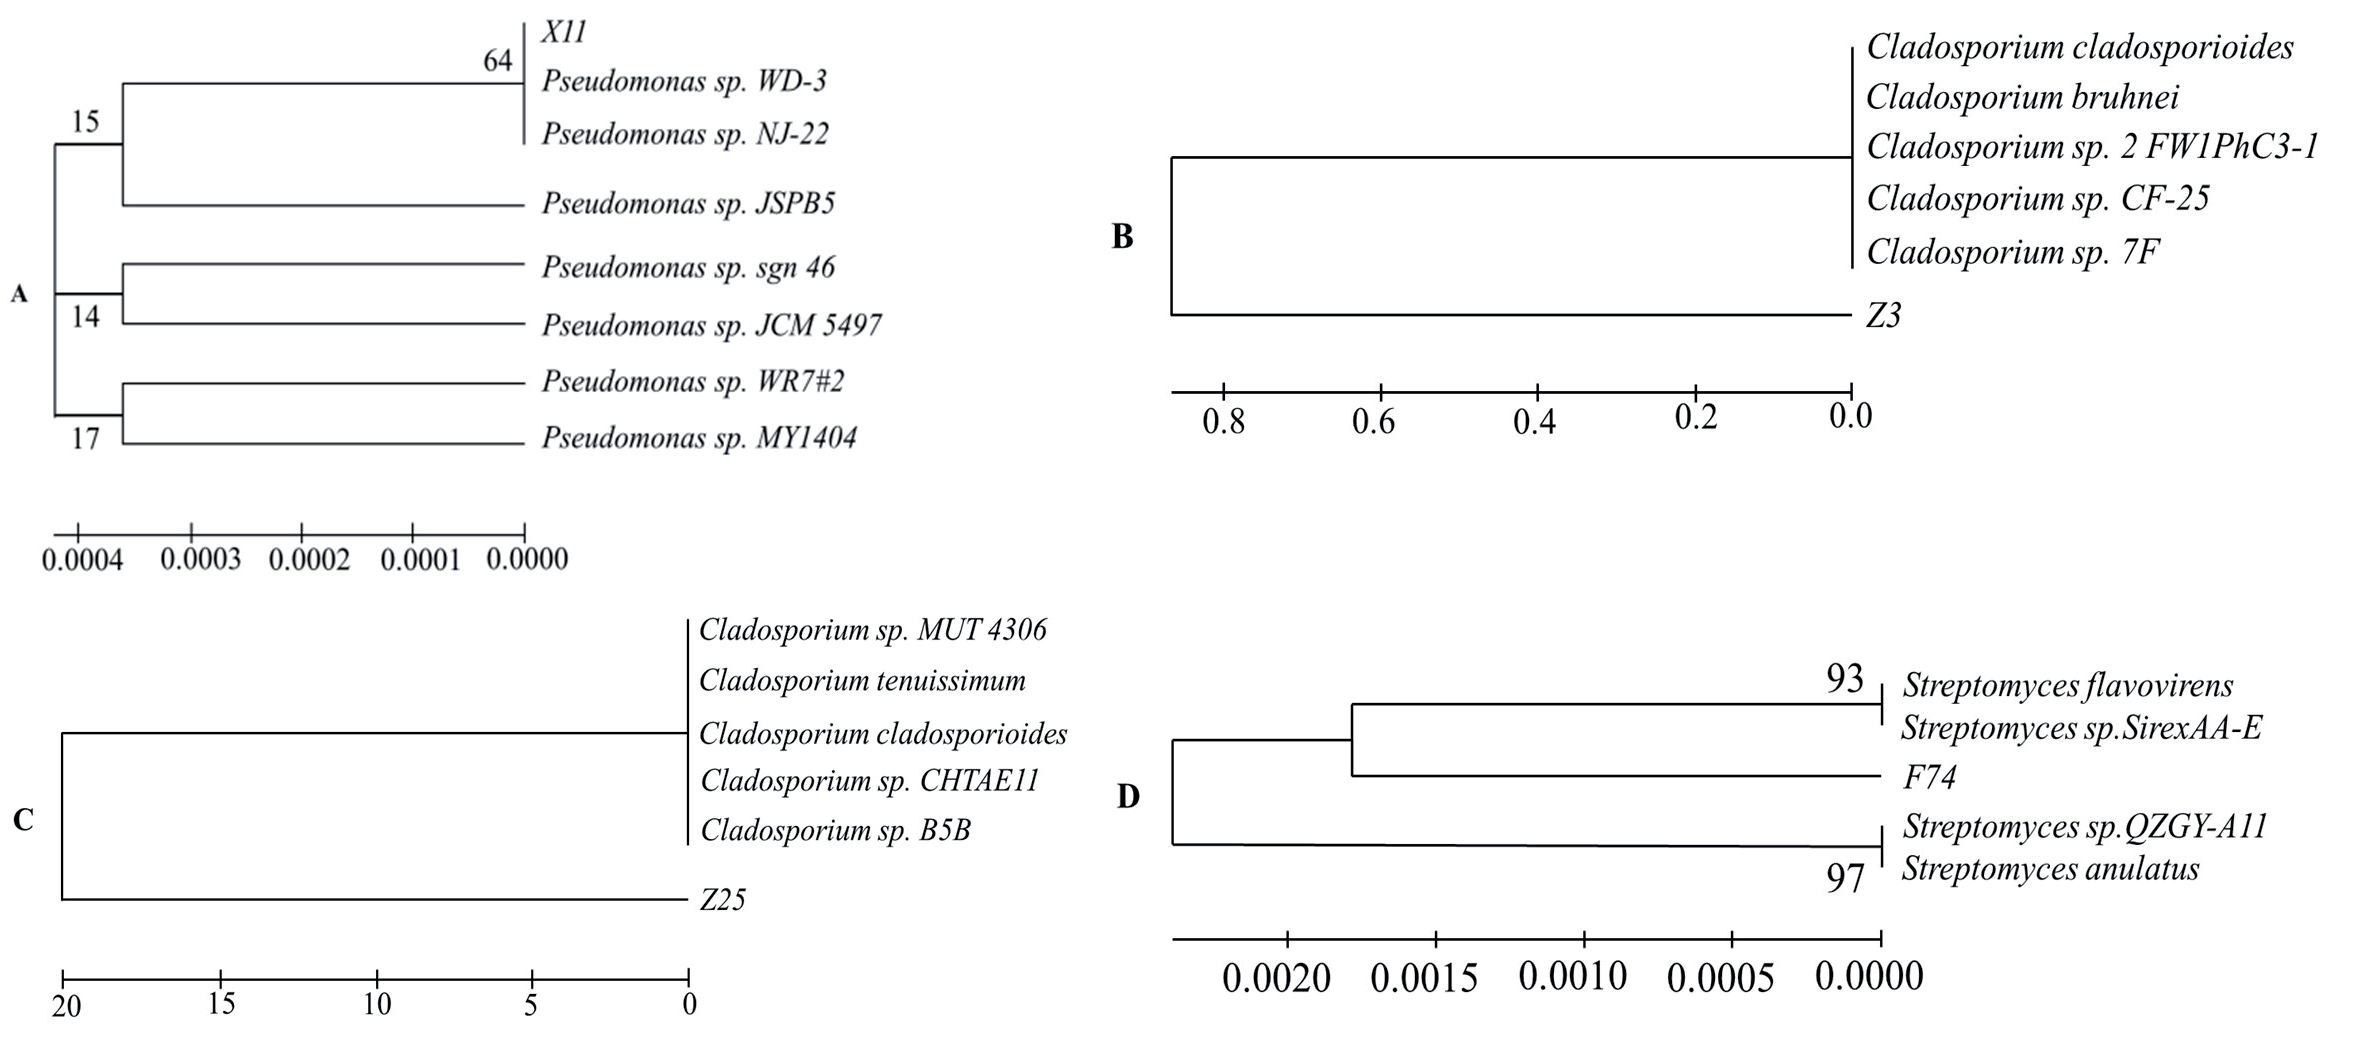
The sequence lengths of the amplified products of Bacteria X11, Fungi Z3, Fungi Z25, and Actinobacteria F74 were 1393 bp, 1686 bp, 568 bp, and 1408 bp, respectively, which were consistent with the expected size of the amplified fragments. The measured sequences were compared in the Genbank database to find their homologous sequences, and the results are shown in Table S1. Strain Pseudomonas sp. sgn 46 was found to share up to 100% homology with bacterium X11, and strain Cladosporium cladosporioides strain TXJ13021 was found to share up to 100% homology with fungus Z3. Strains of Cladosporium sp. MUT 4306, Cladosporium cladosporioides strain M61, Cladosporium cladosporioides strain CFP14, and Cladosporium sp. CHTAE11 showed up to 100% homology with the fungus Z25 with up to 100% homology. Various strains of Streptomyces spp. documented in the GenBank database showed more than 99% homology with Actinomyces F74. The corresponding phylogenetic trees based on this comparison are presented in Fig. 4. It was finally determined that Bacteria X11 belongs to the Pseudomonas sp., Fungi Z3 and Fungi Z25 belong to the Cladosporium sp., and Actinobacterium F74 belongs to the Streptomyces sp.
Mixed Antagonistic Effects of the Candidate Strains
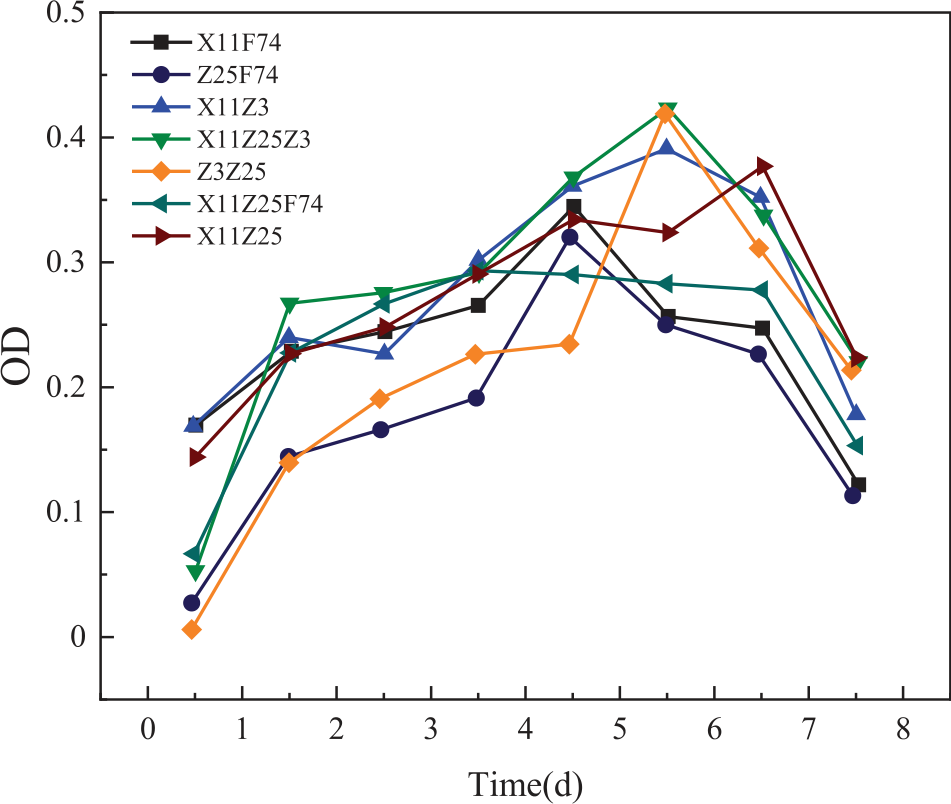
Antagonism tests on the four strains identified revealed antagonistic reactions between strains Z3 and F74, but not between the other strains (Table 1). Seven groups of mixed bacteria were finally obtained as X11F74, Z25F74, X11Z3, X11Z25, Z3Z25, X11Z3Z25, and X11Z25F74 (Fig. S1). Among them, combination X11Z25F74 reached the peak of growth on day 4 and had the fastest growth among all the combinations, while combination X11Z25 was the slowest growth among all the combinations, where combination X11Z25Z3 had the largest growth OD of 0.421 and combination X11Z25F74 had the smallest growth OD of 0.298. In the later stages of incubation, due to nutrient deprivation, the bacteria begin to autolize and the turbidity of the culture solution begins to decrease.
Differences in Enzyme Activity of Mixed Bacteria
From Fig. 2, comparing the enzyme activities of different mixed bacteria, it can be found that X11F74 has the best promotion effect on filter paper degrading enzyme, CMC degrading enzyme, and microcrystalline cellulase, with the highest enzyme activity of 0.327 IU/g, 1.312 IU/g, and 0.289 IU/g, which indicated that the degradation of cellulose was optimally degraded by X11F74. All three enzyme activities of the mixed bacterium X11F74 were greater than those of any of the single bacteria in its fractions, suggesting a synergistic effect of bacteria X11 and F74. It was inferred that the mixed culture of strains could improve the enzyme activity, and the advantage of mixed bacteria for cellulose degradation over single bacteria was obvious. Combined with the above analysis, the mixed bacterium X11F74 is the advantageous low-temperature bacterial group for cellulose degradation.
Study on the Optimal Enzyme Production Conditions of Candidate Colony X11F74
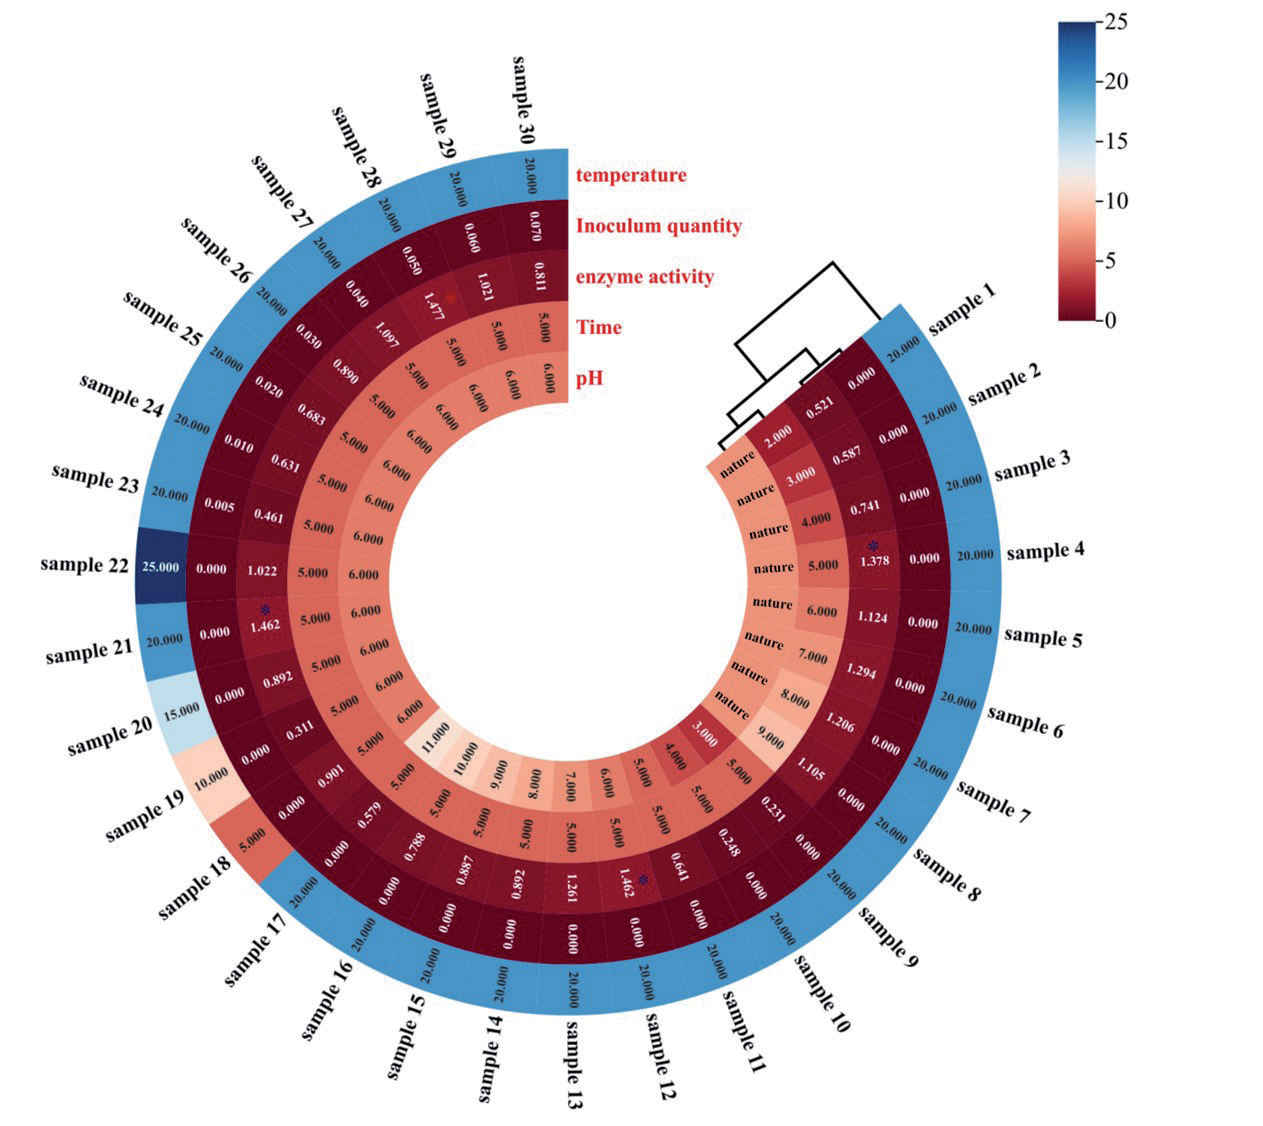
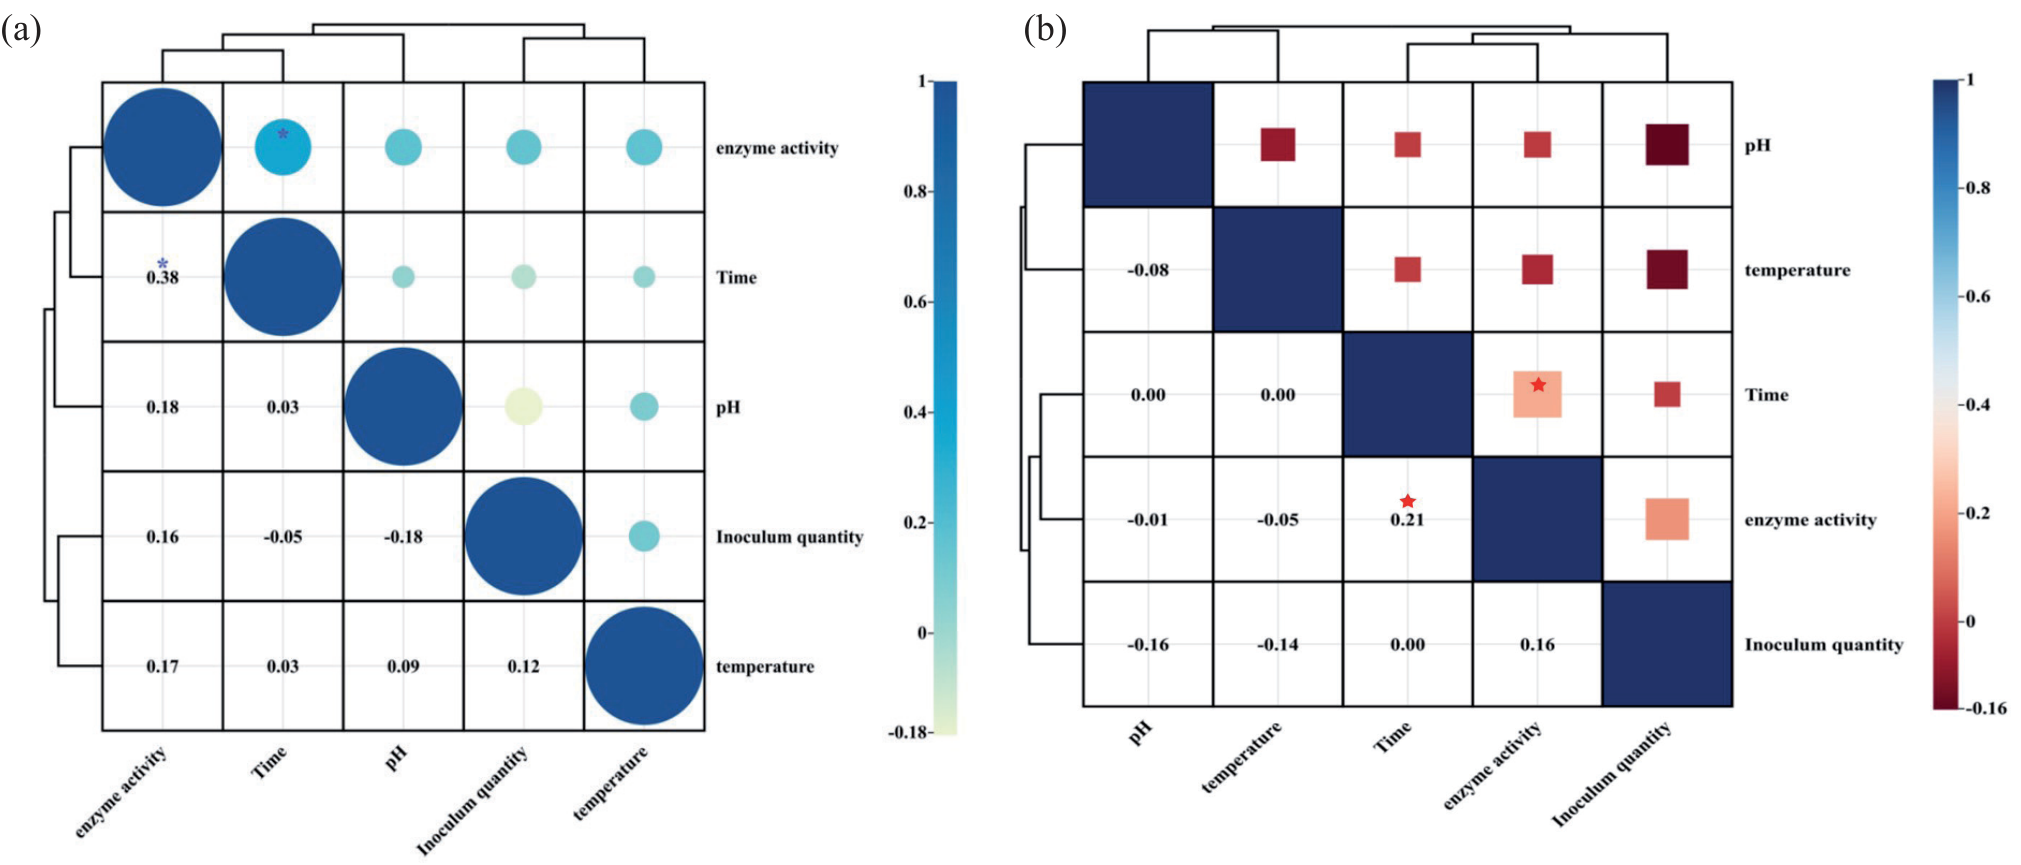
The effect of single factors on the optimal enzyme production conditions of X11F74 is shown in Fig. 5. With different incubation times, X11F74 produced the best enzyme at 5 d of incubation with an enzyme activity of 1.378 IU/g. With different pH, X11F74 produced the best enzyme at pH 6 with an enzyme activity of 1.462 IU/g. The CMC degrading enzyme activity was more stable in the range of 6.0 to 9.2 compared to pH less than 6, suggesting that X11F74 is acid-sensitive and somewhat alkali-resistant, which may be due to the resistance of proteases isolated from Streptomyces and Pseudomonas spp. to alkaline stress [40, 41]; with different temperatures, X11F74 produced the best enzyme at 20ºC with an enzyme activity of 1.462 IU/g; the best enzyme production was achieved by X11F74 at an inoculum level of 5% with an enzyme activity of 1.477 IU/g at different inoculum levels. Due to the excessive addition of bacteria, the nutrients within the medium began to be scarce, affecting the normal growth of the bacteria, and their enzyme activity instead decreased. In summary, the highest enzyme activity of the mixed bacterium X11F74 was observed under the conditions of a 5 d incubation time, an initial pH of 6, an incubation temperature of 20ºC, and an inoculum volume of 5%. Under the optimal enzyme-producing conditions, it was inoculated in the liquid medium with filter paper as the only carbon source to explore its practical application effect under the optimal conditions, and the results are shown in Table 2, and the degradation rate of filter paper could reach 22.84%. Fig. 6a) shows the correlation matrix between the enzyme-producing activity of the mixed bacterium X11F74 and the environmental factors, and the results show that the enzyme-producing activity of the mixed bacterium X11F74 has the strongest correlation with the time factor. Meanwhile, this study screened about 60 pieces of literature about low-temperature cellulose-degrading bacteria in recent years and investigated the correlation between enzyme activity and environmental factors, and the results were shown in Fig. 6b), which found that the microbial enzyme-producing activity was most strongly correlated with the time factor, which verified the results of the correlation matrix study of this experiment. This provides a theoretical basis for the practical application of the mixed bacterium X11F74, which can still better improve the composting efficiency by reasonably applying the key factor of good incubation time when other conditions are difficult to fully satisfy.
Discussion
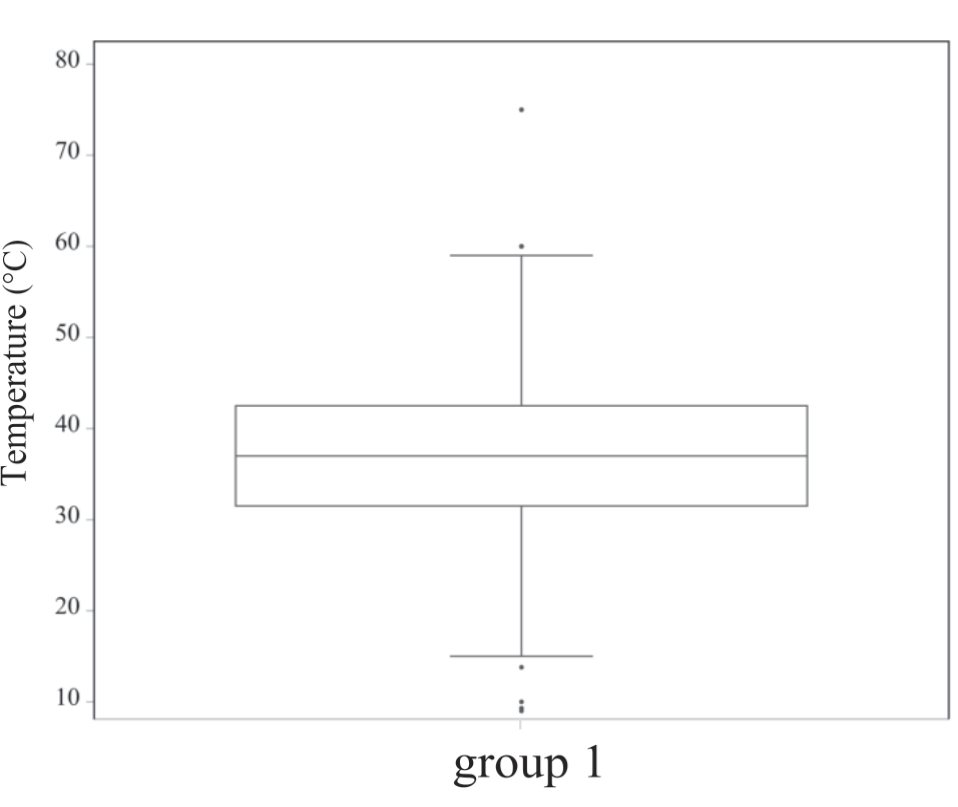
In this study, a large amount of literature on microbial enzyme production in recent years was reviewed, and 40 papers were selected and statistically analyzed through a box plot as shown in Fig. S2. Most of the optimal temperatures for microbial enzyme production were concentrated between 32ºC and 43ºC, and there were fewer studies related to low-temperature cellulose-degrading bacteria, which highlighted the urgency of studying the enzyme production of low-temperature degrading bacteria. Therefore, this study involved the isolation of four strains of low-temperature cellulose-degrading bacteria with high degradation ability from mixed compost derived from straw and livestock manure in cold regions. We hypothesize synergistic interactions among diverse strains during composting, collectively contributing to the degradation of cellulosic materials, and achieving efficient cellulose degradation. Following the initial screening of the four strains, an antagonism test was conducted, and the non-antagonistic single strains were mixed. The growth and enzyme activity of the resultant mixed bacteria were studied, revealing mixed bacteria X11F74 produced the best enzyme effect with more growth and faster growth. A comparison of the enzyme activities of the single bacteria with those of the mixed bacteria X11F74 revealed that all three enzyme activities of the mixed bacteria X11F74 were greater than those of any of the single bacteria in its components. The important effect of synergistic interactions between microorganisms in composting on cellulose degradation has been demonstrated in previous studies. In a study of experimental composting of corn stover and cattle manure by Meng et al. [42], it was found that the degradation rate of cellulose in compost was significantly increased by the synergistic interaction between microorganisms. Han et al. [43] found that β-glucosidase-producing bacteria and fungi synergistically drive cellulose degradation and increase the degradation rate during corn stover composting. Therefore, we conclude that the enzyme activity between both Bacteria X11 and Actinobacteria F74 is enhanced through synergistic action, which effectively improves cellulose degradation efficiency. The optimal conditions for enzyme production by the mixed bacterium X11F74 were found to be 5 d of incubation time, initial pH of the medium at 6, incubation temperature at 20ºC, and an inoculum size of 5% by a one-factor variant test, and the degradation rate of the mixed bacterium under the optimal conditions was 22.8 %. In addition, based on the status of change in the CMC degrading enzyme activity of the mixed bacteria, it can be inferred that the mixed bacteria belong to the cold-resistant rather than cold-loving bacteria, which are sensitive to acidity and have a certain degree of alkali resistance.
Fig. 6.
a) Pearson correlation matrix between enzyme-producing activity of the hybrid bacterium X11F74 and environmental factors. b) Pearson correlation matrix between low-temperature cellulose-degrading bacteria and environmental factors.
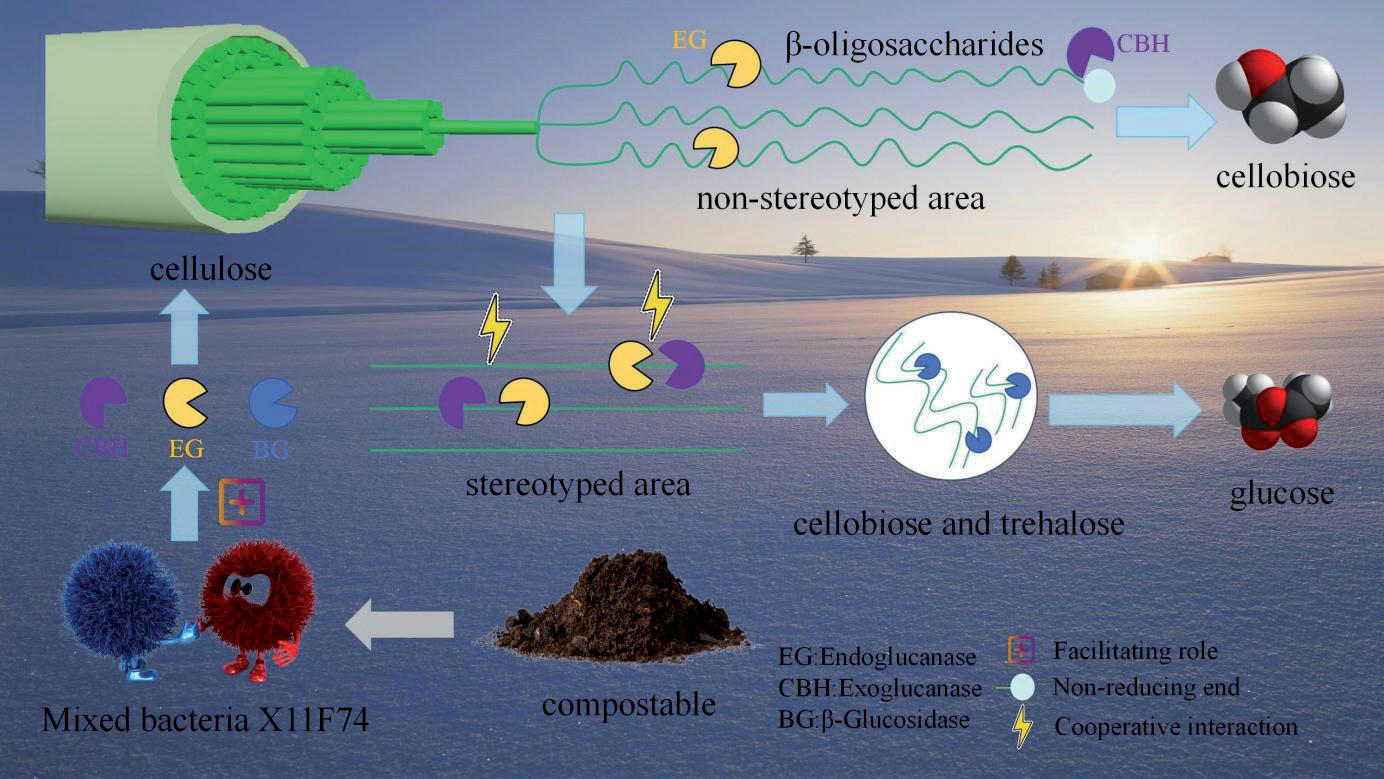
Taken together, the mechanism of cellulose degradation by the mixed bacteria X11F74 was investigated. Mixed bacterium X11F74 increased the activity of secreted cellulase through synergistic action, and cellulase was used to hydrolyze cellulose. The hydrolysis process of cellulase is a joint action of endoglucanase, exoglucanase, and β-glucosidase. Firstly, endoglucanase breaks down the β-1,4 glycosidic bond inside the non-crystalline region of cellulose molecule into short β-glucooligosaccharide, and then exoglucanase reacts with its non-reducing end to decompose the β-oligosaccharides into fibrous disaccharides in disaccharide units; then, endoglucanase and exoglucanase carry out synergistic action to decompose partially degraded cellulose to generate fibrous disaccharides, and fibrous trisaccharides, and other oligosaccharides; finally, it is broken down into glucose under the action of β-glucosidase to complete the hydrolysis process. The degradation mechanism is presented in Fig. 7.
The optimum growth temperature of Bacillus agave from soil screened by Malik et al. [44] was 37ºC, and the optimum pH was 7.0, in comparison to which the mixed bacterium X11F74 is better suited for cellulose decomposition at lower temperatures and higher acidity. In comparison to an Aspergillus sydowii isolated by Matkar et al. [45] with an optimal inoculum quantity of 10% and an optimal incubation time of 6 d, the optimal inoculum quantity of the mixed bacterium X11F74 was smaller and the optimal incubation time was less. Therefore, the mixed bacterium X11F74 obtained in this experiment was superior. In addition, cellulose-degrading bacteria are of great interest for other applications. For example, cellulose-degrading bacteria and pure cultures for the preparation of microbial fuel cells are capable of generating electricity directly from cellulose as an electron donor. This contributes to the reduction of the use of fossil fuels and to the reduction of greenhouse gases [46]. Lactic acid production using cellulolytic flora in the gut of insects saves resources and costs and protects the environment. These studies indicate that cellulose-degrading bacteria have high utilization value, and we look forward to subsequently the further excavation of the potential functions of cellulose-degrading bacteria [47-49].
Conclusions
In this investigation, natural compost served as the bacterial source, and cellulose was employed as the only carbon source. Following a sequence of domestication, isolation, purification, primary screening, rescreening, and enzyme activity studies, four strains of low-temperature cellulose-dominant degrading bacteria were ultimately isolated. Molecular biology identified Bacterium X11 as a member of the Pseudomonas sp., while fungi Z3 and Z25 were assigned to the genus Cladosporium sp., and Actinomycetes F74 were attributed to the Streptomyces sp. Using an antagonism assay, the strains without antagonism were amalgamated and an examination of the mixed bacterial growth and enzyme activity ensued. The resultant analysis disclosed that the filter paper degrading enzyme activity of the mixed bacteria X11F74 measured 0.327 IU/g, CMC degrading enzyme activity reached 1.312 IU/g, and microcrystalline cellulose enzyme activity registered at 0.289 IU/g. The three enzyme activities were significantly better than the other combinations and significantly higher than any of the single bacteria in their constituents, indicating the synergistic effect of X11 and F74, thus identifying the mixed bacterium X11F74 as the best degrading bacterium. Furthermore, the optimal conditions for enzyme production by the mixed bacteria were determined as follows: an incubation time of 5 d, an initial medium pH of 6, an incubation temperature of 20ºC, and an inoculum of 5%. The mixed bacterium X11F74 can indeed be applied to low-temperature compost as a low-temperature efficient cellulose degrading bacterium to promote cellulose degradation. However, the existing literature lacks comprehensive insights into the specific interaction mechanisms governing mixed bacteria. We look forward to the next step of further research on the mixed bacterium from the aspect of molecular cloning and so on.