

Introduction
Walnuts (Juglans regia L.), recognized as one of the world’s four major dried fruits alongside almonds, cashews, and hazelnuts, are also a key component of China’s woody oil crops. They are esteemed for their rich nutritional value and health benefits, making them popular among consumers worldwide [1]. In recent years, China has introduced several policies aimed at boosting the supply of healthy, high-quality edible oils while safeguarding national grain and oil security. These measures have spurred significant growth in the walnut-based woody oil industry [2]. Today, China boasts the largest global walnut cultivation area, spanning 3.33 million hectare [3]. Despite this expansion, challenges have emerged. As walnut planting areas have grown, so has farm management’s complexity. Notably, there is a lack of emphasis on scientific fertilization practices [4]. Farmers often prioritize nitrogen and phosphorus over potassium, creating an imbalance in soil nutrients. Furthermore, annual activities such as pruning and harvesting remove substantial amounts of potassium from orchards, leading to their depletion in the soil and negatively impacting both yield and quality [5]. Potassium, essential for plant growth, supports critical functions, including cell osmotic pressure regulation, stomatal movement, enzyme activity, photosynthesis, assimilate transport, and plant resilience against various stresses [6]. A potassium deficiency can severely impair these processes, resulting in poor leaf health, suboptimal nutrient uptake, hindered root development, reduced biomass, and lower fruit yield and quality. Addressing the issue of potassium deficiency is crucial. Research into how plants absorb and utilize potassium under low-potassium conditions and studies on crop growth and tolerance under potassium stress offer promising solutions to mitigate soil potassium shortages.
While international research on walnuts predominantly focuses on genetic breeding, nutrition, chemical composition, and utilization, there remains a gap in understanding walnut nutrient stress and its response mechanisms [7]. This study aims to investigate the impact of potassium deficiency on walnut seedling’s growth and physiological characteristics, exploring their adaptability and underlying mechanisms under potassium-stressed conditions. The insights gained will provide a scientific foundation for selecting resilient walnut varieties and improving fertilization strategies, thereby supporting the sustainable development of the walnut industry.
Materials and Methods
Experimental Materials and Design
Chongqing Yulu Forestry Development Co., Ltd. provided the experimental material, comprising “Yucheng 1” walnut seedlings. In late November 2018, walnut seeds underwent cold stratification in the sand within the Chongqing Academy of Forestry Sciences greenhouse. In early February 2019, the stratified seeds were sown into seedling beds filled with a substrate mixture (peat: yellow subsoil: perlite = 5:4:1) and managed according to standard protocols [8].
In early April 2019, healthy and uniformly grown seedlings (approximately 20 cm tall and 3 mm in ground diameter) were selected, carefully washed with deionized water, and transplanted into ceramic pots filled with clean quartz sand (20 cm in height and 18 cm in diameter), containing 5 kg of sand per pot, for a total of 90 plants [9]. Following transplantation, an acclimatization period of 15 days was observed, during which only regular watering practices were applied. Subsequently, the seedlings were randomly assigned to three groups, each comprising 30 pots, receiving different nutrient solutions based on Hoagland’s solution: Control (CK), full nutrient solution; Moderate potassium deficiency (MK), with potassium reduced to 50% of the control; Severe potassium deficiency (SK), with no added potassium [10].
During the cultivation period, the volume of nutrient solution applied was determined from preliminary experiments, and the nutrient solution was evenly distributed to the roots using a spray bottle every five days at a rate of 100 mL per pot. Regular watering was maintained throughout the experiment. Growth and physiological indicators were measured every 15 days [11, 12]. An experiment scheme of element deficiency in walnut seedlings is shown in Table 1.
Experimental Methods
Biomass and Specific Root Area Measurement
Five plants were randomly sampled from each treatment group for analysis, serving as replicates. The whole plants were collected, and the aboveground parts and roots were separated, washed with deionized water, and dried at 80°C until constant weight. Dry weights were measured using an electronic balance with a precision of 0.0001 g. The root-shoot ratio was calculated as the roots’ biomass divided by the aboveground parts’ biomass. The root surface area was measured using Canada’s WinRHIZO root analysis system. Specific root area (cm²/g) refers to the root surface area per unit dry weight, calculated as follows: Specific root area = root surface area / dry weight [13, 14].
Root Activity Assay
Root activity was measured using the TTC (2, 3, 5-triphenyltetrazolium chloride) method. The absorbance was measured at a wavelength of 485 nm using a Shimadzu UV2600 spectrophotometer (Shimadzu Inc., Japan). A control sample (adding sulfuric acid first to inhibit the TTC reduction caused by dehydrogenase in plant roots, with the rest of the procedure being the same) was used as the reference to determine the absorbance. The root activity was then calculated by referring to the standard curve [15, 16].
Table 1.
Experiment scheme of element deficiency of walnut seedlings.
Photosynthetic Pigment Content Determination
Photosynthetic pigment content in leaves was determined using the acetone-ethanol extraction method (acetone: ethanol: water = 4:5:1). For each sample, the second and third fully expanded leaves from the base of the plant were selected, and 0.1 g of leaf tissue was extracted in 10 mL of mixed solvent for 24 hours. The extract was used for colorimetric analysis at wavelengths of 470 nm, 645 nm, and 663 nm to calculate chlorophyll a (Chl a), chlorophyll b (Chl b), and carotenoid (Car) contents. The ratio of chlorophyll a to b (Chl a/b) was calculated as the ratio of chlorophyll a to chlorophyll b [17, 18].
Photosynthetic Parameters Measurement
Measurements were taken between 9:00 and 11:00 AM on sunny days. Photosynthetic parameters such as net photosynthetic rate (Pn), stomatal conductance (Gs), and transpiration rate (Tr) of the seedlings were measured using the Li-6800 photosynthesis measurement system (LI-COR Inc., USA). During the measurement, the light intensity inside the leaf chamber was set to 1200 µmol·m⁻²·s⁻¹, the CO2 concentration was the same as the ambient atmospheric concentration, and the leaf temperature was between 25 and 30°C. Water use efficiency was expressed as the amount of CO2 fixed per unit of water consumed, calculated as the net photosynthetic rate divided by the transpiration rate [19, 20].
Endogenous Hormone Content Determination
Endogenous hormones, including auxin (IAA), cytokinin (CTK), and abscisic acid (ABA), were extracted from leaves following the method described [21]. Hormones were detected using an Agilent 1100 high-performance liquid chromatography system (Agilent Technologies Inc., USA). Detection wavelengths were set at 210 nm for IAA and ABA and 265 nm for CTK. The injection volume was 20 μL, and the mobile phase consisted of methanol: acetonitrile: phosphate buffer (pH 3.5) = 15:20:65. Column temperature was set at 35°C, and flow rate at 10 mL/ min. Ethylene was extracted from the leaves according to the protocol [22], and detection was performed using a Shimadzu GC-9A gas chromatograph (Shimadzu Inc., Japan). Detection conditions included an HP-5 column (30×0.25 mm), flame ionization detector (FID), and injection volume of 5 μL. The detector temperature was set at 230°C.
Polyamine Content Determination
Polyamines, including putrescine (Put), spermidine (Spd), and spermine (Spm), were extracted from leaves according to [23]. Detection was carried out using an Agilent 1100 high-performance liquid chromatograph (Agilent Technologies Inc., USA). Detection conditions were as follows: A detection wavelength of 254 nm, an injection volume of 10 μL, a mobile phase consisting of 64% methanol (prepared with ultrapure water), a column temperature of 25°C, and a flow rate of 0.8 mL·min⁻¹.
Results
The Effect of Potassium Deficiency on the Growth of Walnut Seedlings
From Table 2, it can be seen that under potassium-deficient conditions, both the aboveground biomass and root biomass of walnut seedlings significantly decreased compared to the CK treatment, and the decline became more pronounced as potassium deficiency increased and the extension of treatment time. Walnut seedlings continued to grow after being subjected to varying degrees of potassium deficiency stress, but their growth rate significantly decreased compared to the CK treatment, especially in the later stage of treatment (45-75 days). At the end of the treatment (75 days), the aboveground biomass of the MK and SK treatments was 39.3% and 52.5% lower than that of the CK, respectively, with significant differences (P≤0.05); the root biomass of the MK and SK treatments was 21.3% and 24.2% lower than that of the CK, respectively, with significant differences (P≤0.05). Conversely, as the degree of potassium deficiency and the duration of treatment increased, the root-shoot ratio and specific root area of walnut seedlings generally increased. At the end of the treatment, the root-shoot ratio of the MK and SK treatments was 29.9% and 60.8% higher than that of the CK, respectively, with significant differences (P≤0.05); the specific root area of the MK and SK treatments was 15.3% and 16.7% higher than that of the CK, respectively, with significant differences (P≤0.05) [24].
The Effect of Potassium Deficiency on the Root Activity of Walnut Seedlings
As shown in Fig. 1, over the first 30 days, the root activity of walnut seedlings in all treatments significantly increased (P<0.05). The CK treatment remained at a stable level with no significant change (P>0.05), while the MK and SK treatments showed a downward trend, both of which showed a significant increase after 60 days (P≤0.05). Throughout the treatment process, root activity was highest in the SK treatment, followed by the MK treatment, and the lowest in the CK treatment [25]. At 75 days, the root activity of the MK and SK treatments was 16.7% and 40.7% higher than that of the CK, respectively, with significant differences (P≤0.05) [26-28].
The Effect of Potassium Deficiency on the Photosynthetic Pigments of Walnut Seedlings
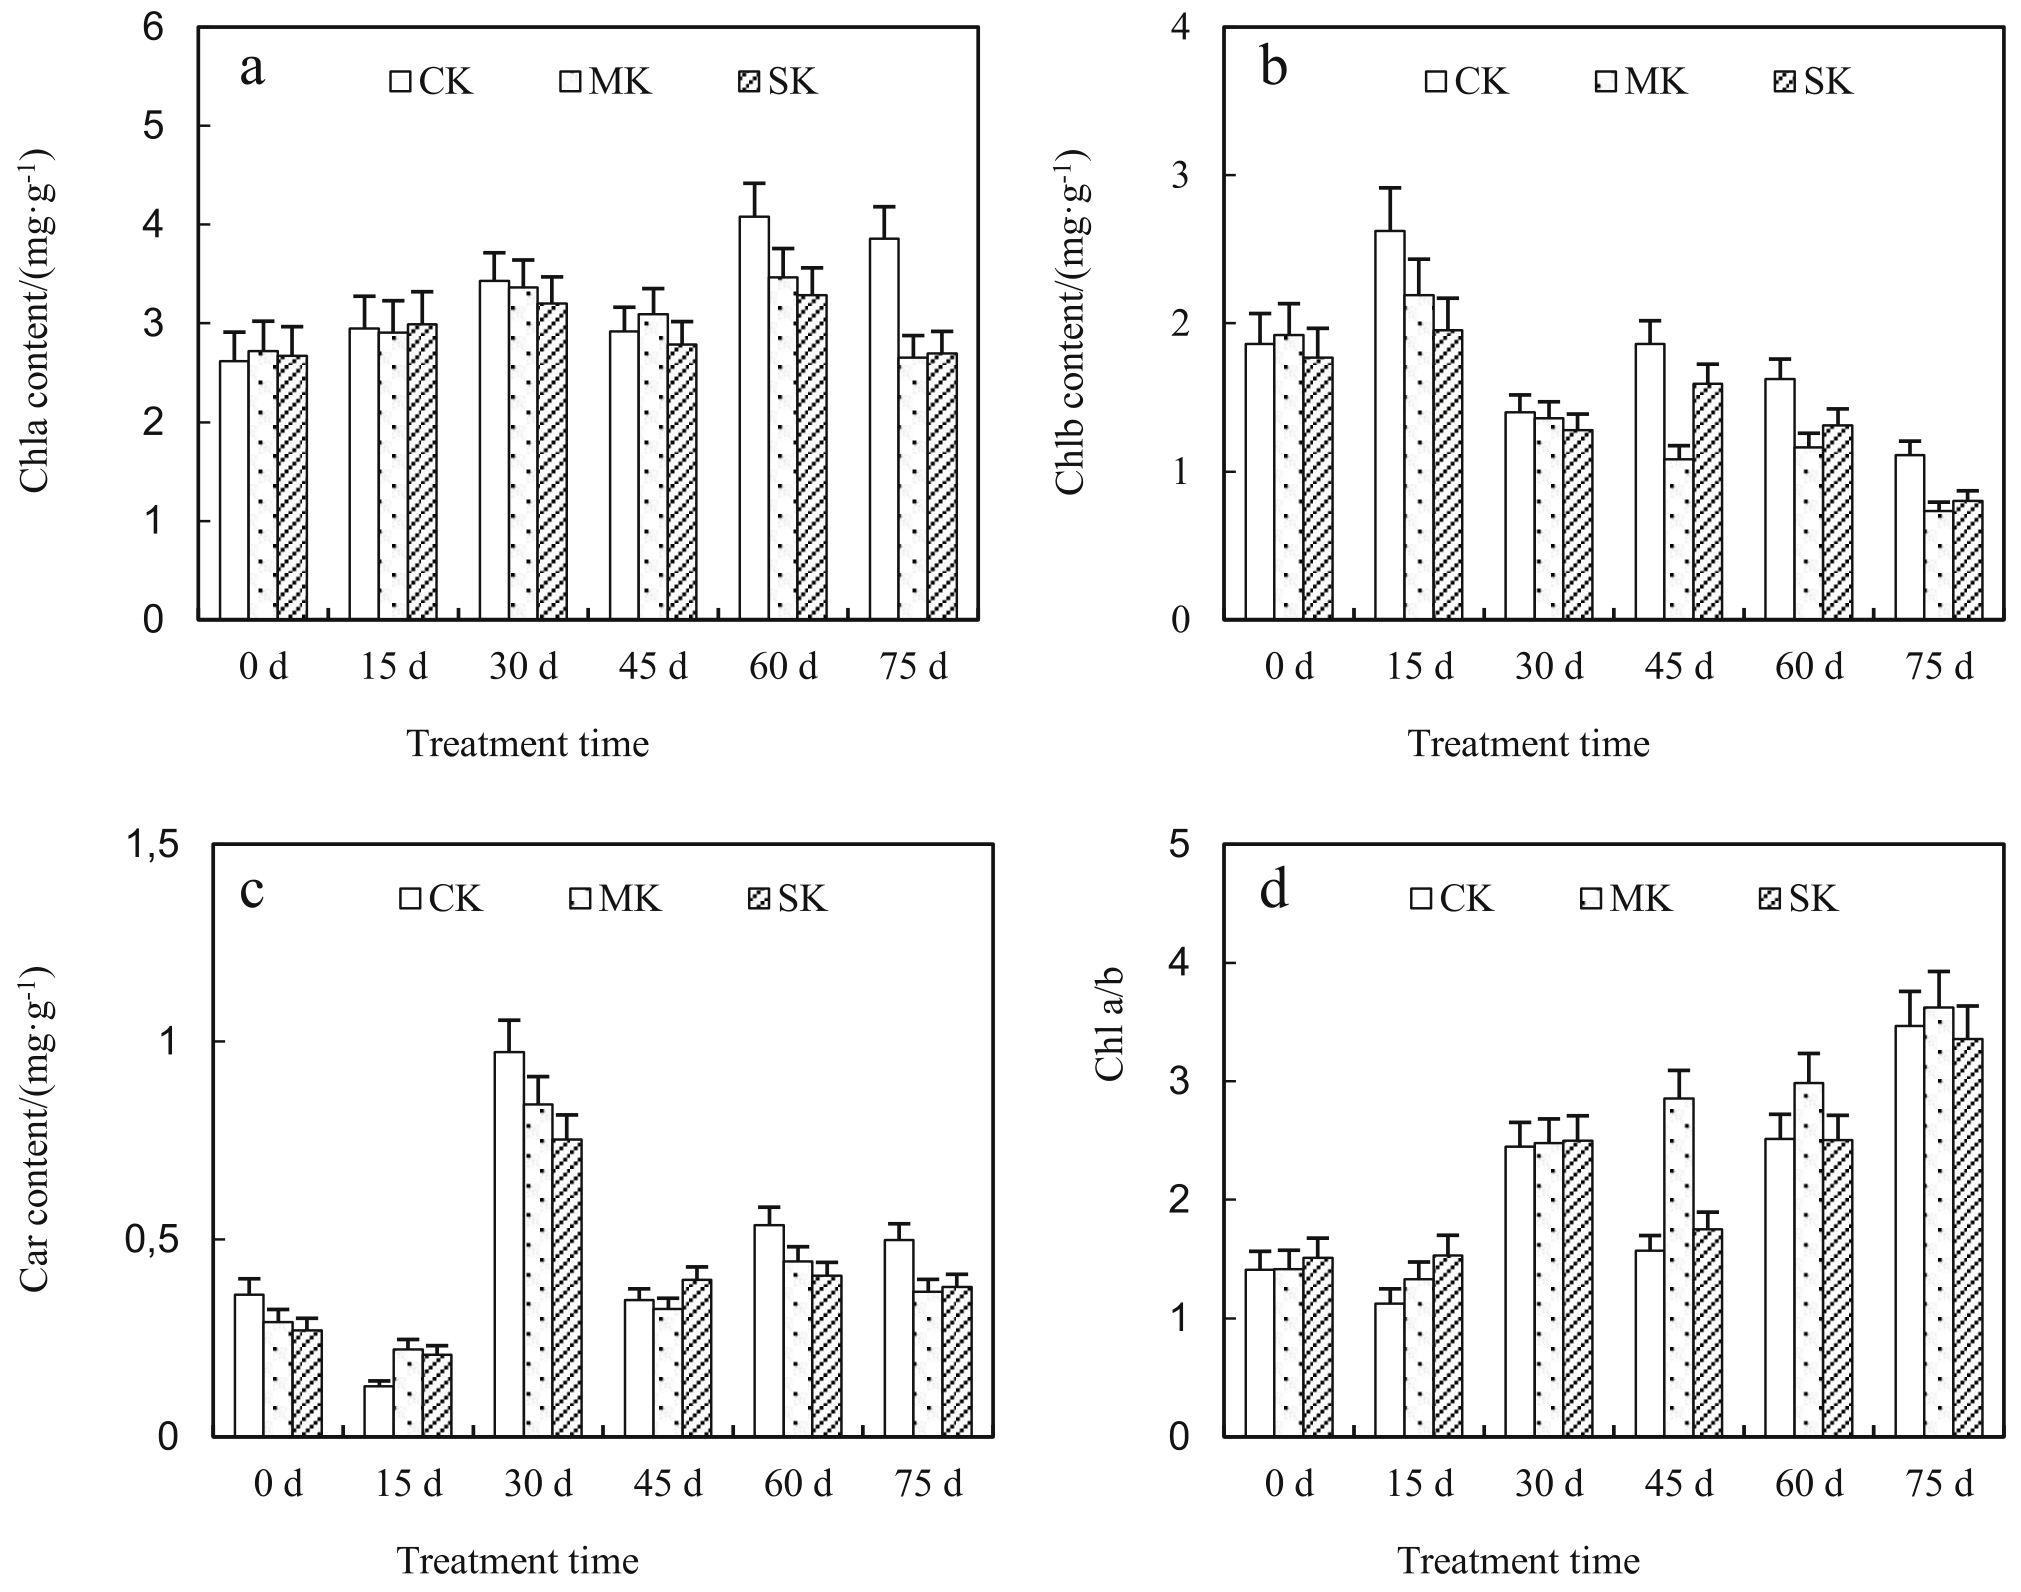
As shown in Fig. 2a), with the extension of the treatment time, chlorophyll a content in the CK treatment generally showed an upward trend, while the chlorophyll a content in the MK and SK treatments increased in the early stage of treatment but significantly decreased in the later stage (P≤0.05). With the extension of treatment time, the chlorophyll b content in all treatments generally decreased (Fig. 2b)), and the carotenoid content in all treatments showed a trend of first increasing and then decreasing (Fig. 2c)). As the treatment time extended, there was no fixed trend in the change of the chlorophyll a/b ratio in the CK treatment, but the MK and SK treatments showed a consistent increase (Fig. 2d)). With the aggravation of potassium deficiency stress, the contents of chlorophyll a, chlorophyll b, and carotenoids in walnut seedlings generally decreased, with the SK treatment having the lowest content, and the differences were significant (P≤0.05). Conversely, the chlorophyll a/b ratio increased, but overall, the MK treatment was higher.
The Effect of Potassium Deficiency on the Photosynthetic Parameters of Walnut Seedlings
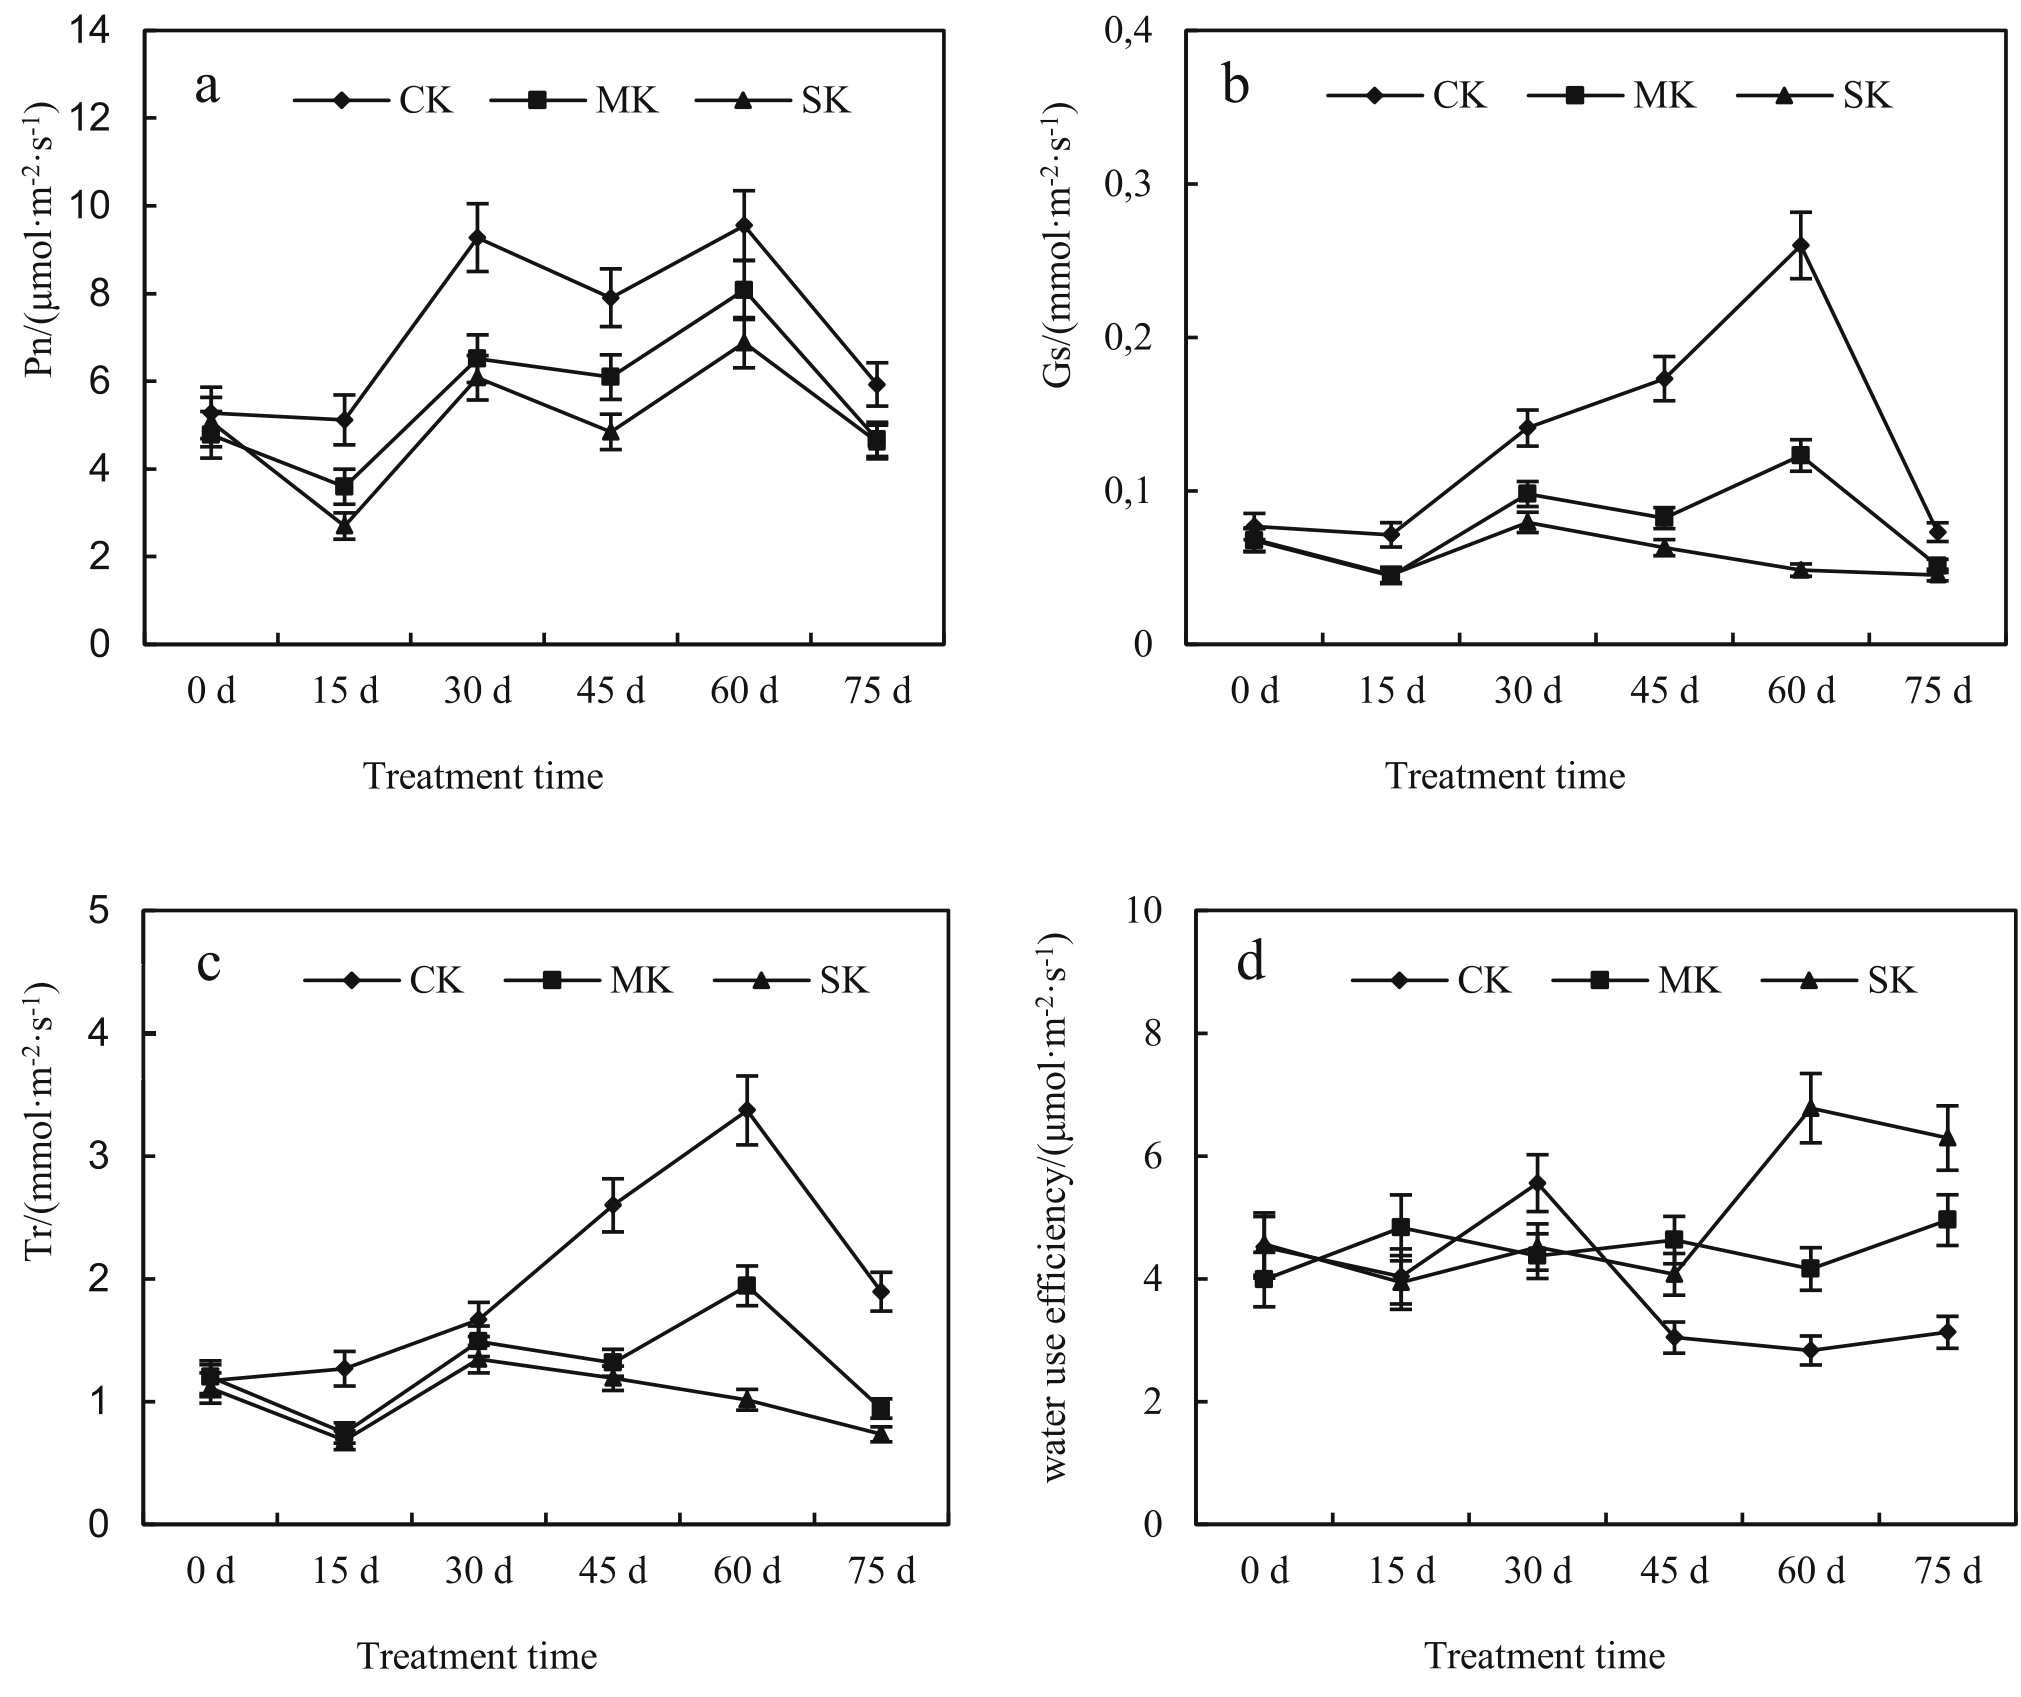
As shown in Fig. 3a), with the extension of treatment time, the net photosynthetic rate of walnut seedlings in all treatments showed a consistent overall trend. The changes in stomatal conductance and transpiration rate were similar between treatments, generally showing an upward trend, but significantly decreased after 60 days (P≤0.05) (Figs. 3b) and 3c)).
Throughout the treatment process, with the aggravation of potassium deficiency stress, the net photosynthetic rate, stomatal conductance, and transpiration rate of walnut seedlings all significantly decreased (P≤0.05). As shown in Fig. 3d), in the early stage of treatment (0-30 days), the water use efficiency of walnut seedlings in all treatments did not change significantly (P>0.05). After 30 days, the CK treatment significantly decreased (P≤0.05), the SK treatment significantly increased (P≤0.05), and the MK treatment showed no significant change (P>0.05). Overall, after being subjected to varying degrees of potassium deficiency stress, the water use efficiency of walnut seedlings improved, and the increase was more pronounced with the aggravation of stress.
The Effect of Potassium Deficiency on the Endogenous Hormones of Walnut Seedlings
As shown in Fig. 4a) and 4b), with the extension of treatment time, IAA and CTK contents in all treatments showed a trend of first increasing and then decreasing. Throughout the treatment process, the IAA and CTK contents were highest in the SK treatment, followed by MK, and lowest in the CK treatment. With the aggravation of potassium deficiency stress, the ABA content in walnut seedlings also significantly increased, with the SK treatment being the highest, followed by the MK treatment, and the CK treatment being the lowest. The differences between treatments were greater in the later stage (60-75 days).
Table 2.
Biomass allocation of walnut seedlings under different treatments (Mean±SE).
As shown in Fig. 4d), from 0 to 30 days, the ethylene content in walnut seedlings under the two potassium deficiency treatments showed an upward trend but significantly decreased after 30 days (P≤0.05), while the CK treatment showed no significant change throughout the treatment. Throughout the treatment process, the ethylene content in the SK treatment was significantly higher than that in the MK and CK treatments (P≤0.05) from 0 to 30 days, but after 30 days, the ethylene content in the SK treatment remained significantly higher than that in the MK treatment, while the CK treatment’s ethylene content was not significantly different from the MK treatment (P>0.05).
The Effect of Potassium Deficiency on Polyamines in Walnut Seedlings
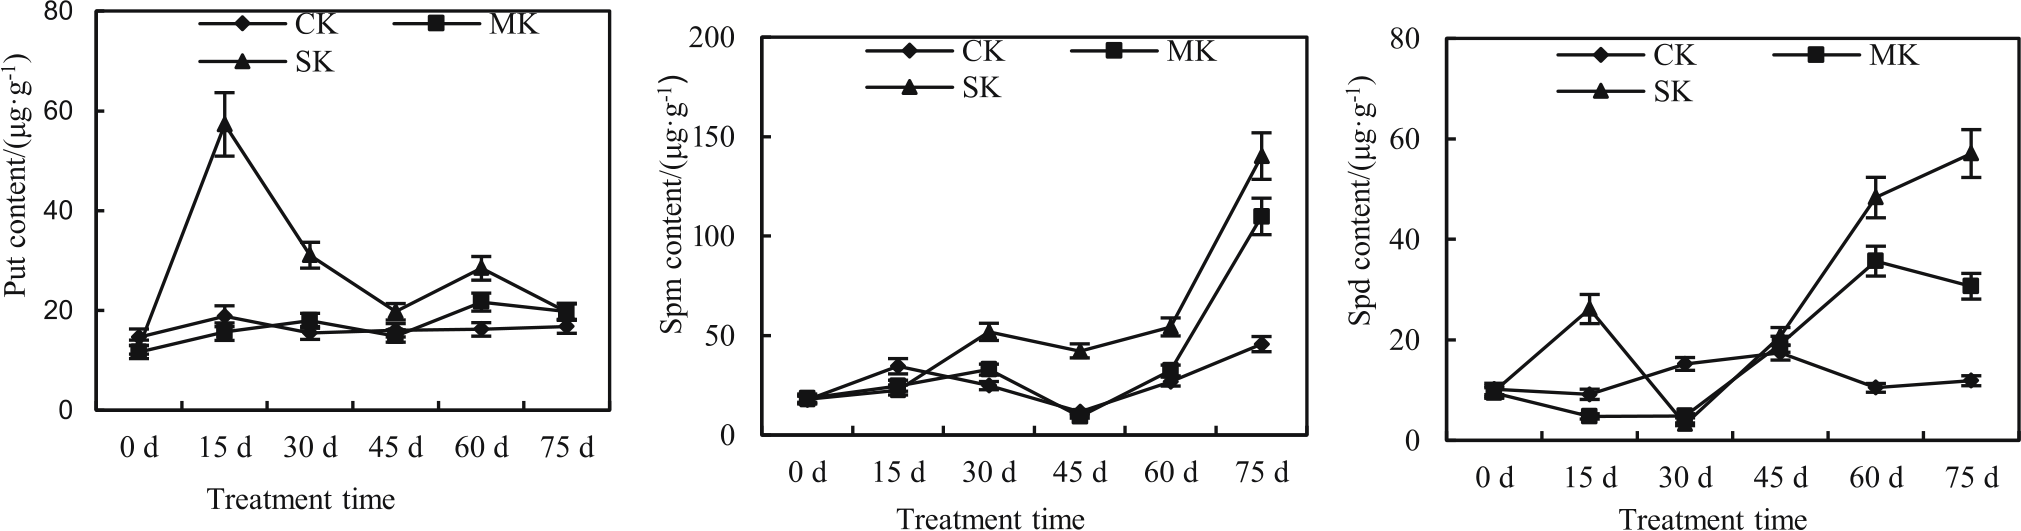
As shown in Fig. 5a), with the extension of the treatment time, there was no significant change in the Put content of walnut seedlings in the CK and MK treatments (P<0.05). However, the SK treatment showed a significant increase in the early stage of treatment (0-15 days) (P≤0.05), followed by a significant decrease (P≤0.05). Overall, throughout the treatment process, the Put content in walnut seedlings significantly increased with the aggravation of potassium deficiency (P<0.05); as shown in Figs. 5b) and 5c), with the extension of treatment time, there was no significant change in the Spm and Spd content of walnut seedlings in the CK treatment. Still, both the MK and SK treatments showed a significant upward trend (P<0.05). Throughout the treatment process, the Spm and Spd content was generally at their highest in the SK treatment, followed by the MK treatment, while the lowest was in the CK treatment, with significant differences (P≤0.05).
Discussion
Potassium is an essential nutrient for plants, but it does not directly participate in the composition of plant tissues. Instead, it primarily functions by participating in physiological metabolic activities, promoting the transport of assimilates and energy transformation within plants. Potassium deficiency in plants can affect the absorption of mineral nutrients such as nitrogen, phosphorus, calcium, and magnesium, as well as the synthesis and transport of assimilates within the plant, which has been confirmed in many plants. This was also the case for walnut seedlings under potassium deficiency conditions. Visually, the walnut seedling’s growth rate and biomass under both potassium deficiency treatments significantly decreased. At the same time, the contents of chlorophyll a, chlorophyll b, and carotenoids in the leaves also significantly decrease, and the decrease becomes more severe with the increase of potassium deficiency. This indicates that long-term potassium deficiency will inevitably affect the absorption and transformation of substances required for chlorophyll synthesis in walnut seedlings, thus affecting chlorophyll synthesis and causing the destruction of the chloroplast photosynthetic apparatus, ultimately affecting photosynthesis. The decrease in plant photosynthetic rate can be divided into two mechanisms: stomatal limitation and non-stomatal limitation. One is the decrease in stomatal conductance, which prevents the supply of CO2, and the other is the decrease in the photosynthetic capacity of mesophyll cells, which reduces their ability to use CO2. The chlorophyll content of walnut seedlings is less affected by potassium deficiency stress in the early stage, but it severely decreases in the later stage, while stomatal conductance and transpiration rate significantly decrease after potassium deficiency stress, which is because the lack of potassium ions directly leads to varying degrees of stomatal closure. This indicates that walnut seedlings are mainly affected by stomatal limitation in the early stage of potassium deficiency stress. As the stress time extends, they gradually shift to the dual influence of stomatal and non-stomatal limitations, which is also the main reason why the photosynthetic rate decreases more significantly in the later stage. Although the photosynthetic activity of walnut seedlings is weakened under potassium deficiency stress, and the biomass of aboveground and underground parts is significantly reduced, with the extension of stress time, the root-shoot ratio and specific root area are significantly improved, especially at the end of the experiment; the root-shoot ratio and specific root area of walnut seedlings under severe potassium deficiency stress are significantly higher than those of the CK treatment by 60.8% and 16.7%, respectively. In addition, root activity also significantly increased after stress. Root activity represents the content of succinate dehydrogenase, which is closely related to respiration, indicating that walnut seedlings adjust themselves under potassium deficiency stress by increasing investment in the root system and also by enhancing physiological activities such as respiration, accelerating the circulation of substances and energy within the body, thereby improving the ability to absorb potassium.
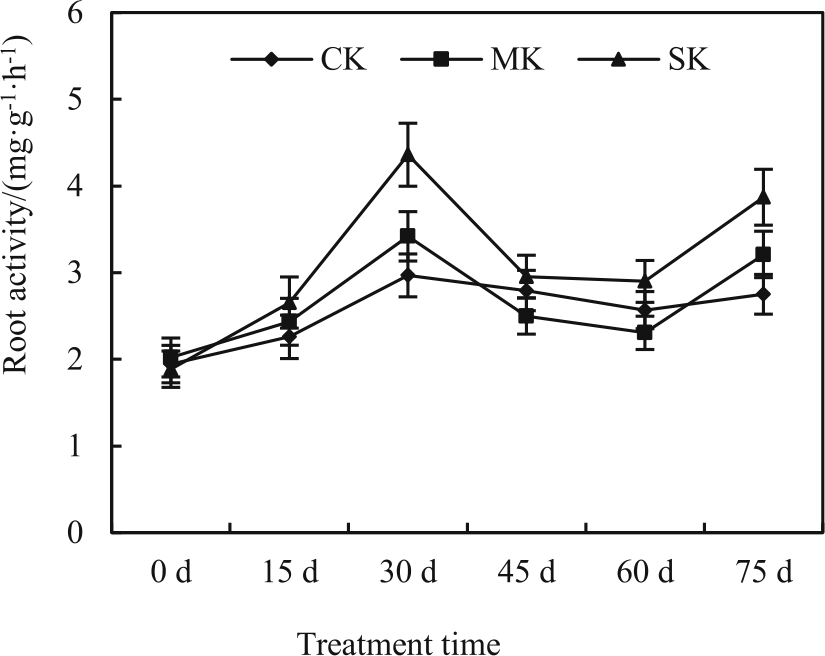
Fig. 2.
The photosynthetic pigment content in the leaf of walnut seedlings under different treatments (Mean±SE).
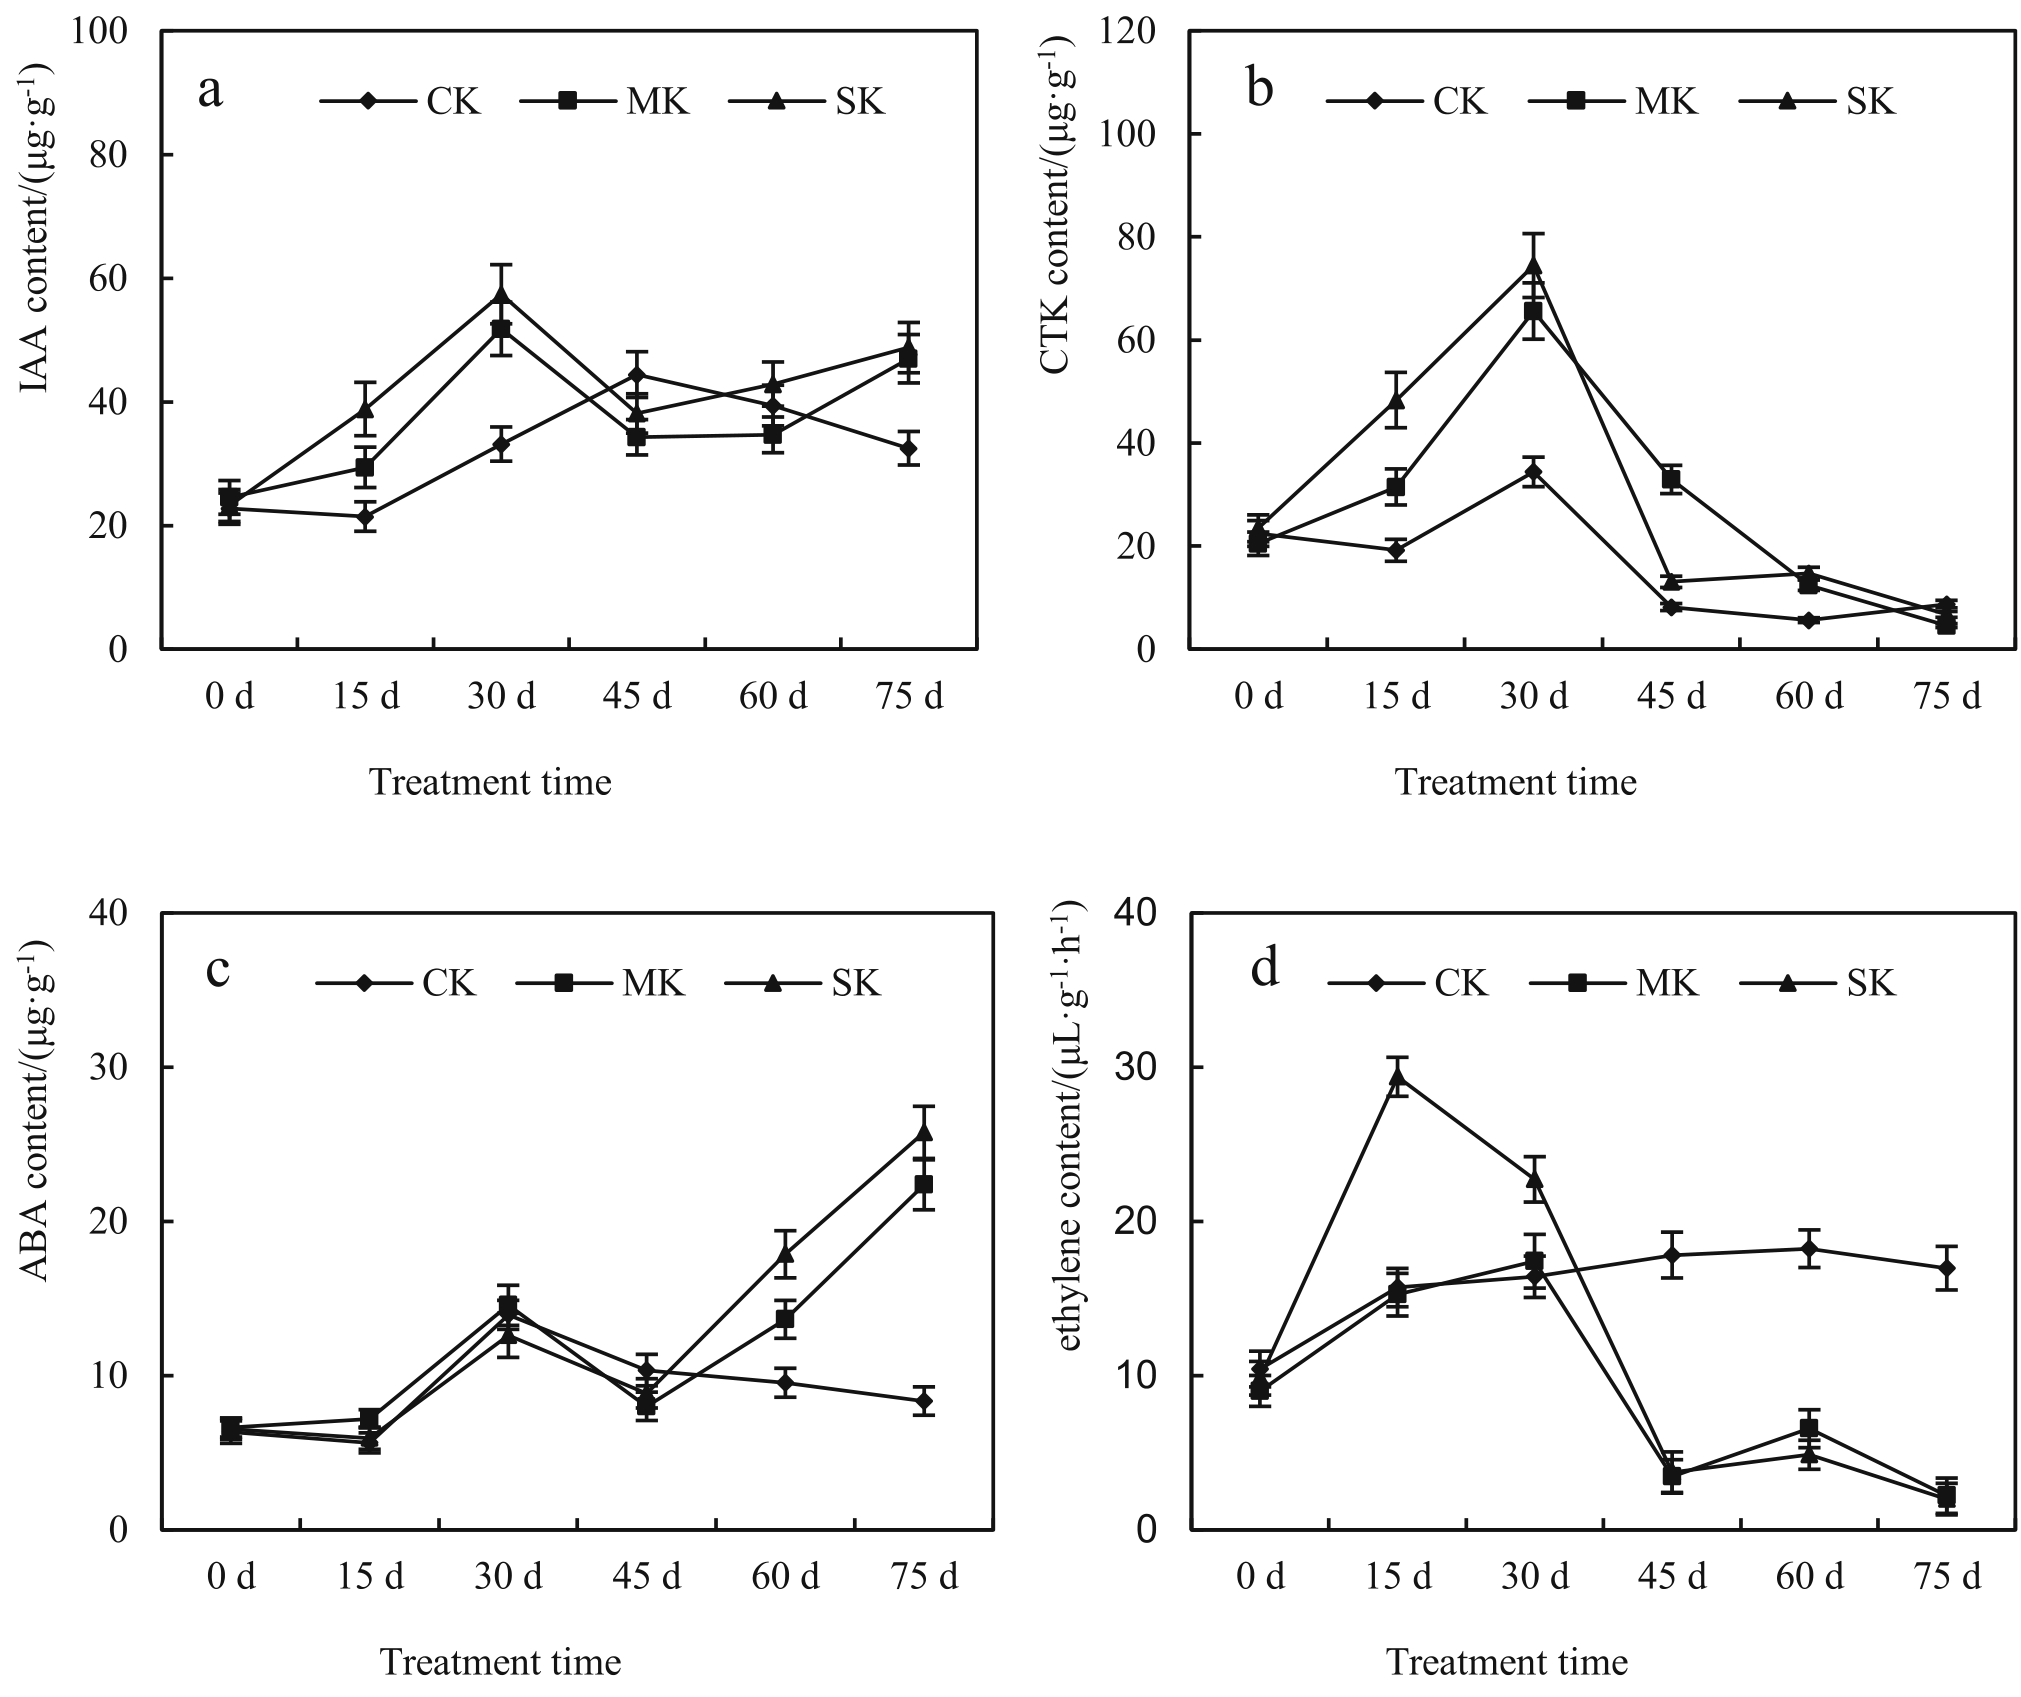
ABA plays a crucial role in plant response to stress, with the closure of leaf stomata closely related to abscisic acid (ABA) and its signaling process. Oosterhuis et al. found that ABA binds to transmembrane receptors on the plasma membrane of guard cells, activating G proteins, which subsequently lead to the release of IP3, triggering the transfer of Ca2+ from the vacuole or endoplasmic reticulum to the cytoplasm. The increase in cytoplasmic Ca2+ concentration inhibits the function of the proton pump, leading to depolarization of the cell membrane and accelerated efflux of cytoplasmic K+, causing the guard cells to lose water and shrink, thereby closing the stomata. Therefore, after walnut seedlings are subjected to potassium deficiency stress, the content of ABA in the body significantly increases and continues to rise with the extension of potassium deficiency time, accompanied by a continuous decrease in stomatal conductance. This also indicates that ABA plays an important role as a signaling substance in walnut seedlings responding to potassium deficiency stress, just as it does in other adversities. At the same time, potassium deficiency can also reduce the turgor pressure of epidermal cells, reducing their force on guard cells and thereby causing stomatal closure. Therefore, under potassium deficiency conditions, the decrease in the photosynthetic rate of walnut seedlings is mainly affected by stomatal limitation. Some studies have also shown that ABA can stimulate ethylene synthesis, and the increase in ethylene can also promote cell aging and cell wall degradation. Hei [20] found in Arabidopsis research that potassium deficiency can increase ethylene production in leaves, affecting the regulation of ABA signaling on stomatal closure. However, this study found that the ethylene content in walnut seedlings under potassium deficiency conditions was consistent with the trend of ABA change in the early stage of treatment (0-30 days) but gradually decreased after 30 days, finally becoming significantly lower than the CK treatment. This may be because long-term potassium deficiency affects the precursors of ethylene synthesis, leading to a reduction in ethylene content in the later stage. At the same time, with the decrease in ethylene synthesis, the speed of plant aging also slows down, which may be another physiological mechanism of walnut seedlings to cope with potassium deficiency stress, but this requires further research.
During the growth process of plants, IAA can promote cell elongation and accelerate nuclear division. CTK mainly acts on the division of cytoplasm, and the effect of CTK on promoting cell division can only be manifested under the presence of IAA. Many scholars believe that potassium deficiency affects the synthesis of IAA, and some studies have also shown that under potassium deficiency conditions, the content of IAA increases. Guo et al. [24] found that exogenous IAA can also increase root growth and promote the absorption of potassium ions under potassium deficiency conditions. Similarly, the content of IAA in walnut seedlings significantly increased under potassium deficiency conditions, and the increase was greater with the increase in stress severity and the extension of time. We determined that this may also be an important response mechanism for walnut seedlings to adapt to potassium deficiency stress, aiming to accelerate cell division and promote the growth of the underground parts to cope with adversity stress. Ding et al. [25] believed that mineral nutrient reduction would decrease the concentration of CTK in the aerial part and root system, thereby reducing the plant’s relative growth rate and root respiration. This study also found that the content of CTK in walnut seedlings significantly increased in the early stage of potassium deficiency stress but gradually decreased over time, which is consistent with the results of most potassium stress studies [26, 27]. CTK can promote the polar transport of IAA. Hence, as the content of CTK decreases, the transport of IAA is also affected, leading to its accumulation in walnut leaves, thereby interfering with normal protein and nucleic acid metabolism processes and potentially inhibiting plant growth [28]. Therefore, under short-term potassium deficiency stress, the increase in the content of IAA and CTK is beneficial for accelerating cell division, improving potassium utilization, and alleviating stress. However, long-term potassium deficiency will lead to an imbalance in the levels of these two substances, which is not conducive to plant growth. This also indicates that IAA and CTK, as growth hormones, are important substances for walnut potassium deficiency stress signal transmission and promoting the absorption and transport of potassium by the root system.
Many studies suggest that when plants are exposed to stresses such as salinity, drought, cold injury, heat injury, heavy metals, and mechanical damage, they regulate the synthesis and catabolism of polyamines and influence the dynamic balance through various signaling transductions to resist the harm caused by adversity stress. Richards et al. [29] first reported the phenomenon of a large accumulation of Put in barley leaves under potassium deficiency stress. Subsequent experiments also confirmed that potassium deficiency can cause an increase in Put content, as well as other nutritional stresses, such as magnesium deficiency, ammonia excess, and calcium excess, which can lead to an increase in the content of polyamines and arginine decarboxylase activity in plants [30, 31]. Some studies have also shown that the content of polyamines in plants can decrease under stress. For example, the content of polyamines in tomatoes gradually decreases with the extension of salt stress time [32]. Under low night temperatures, the content of Put, Spd, and Spm in melon fruits significantly decreases [33]. Similarly, under potassium deficiency stress, the content of Put, Spd, and Spm in walnut seedlings also significantly increases, and the increase is more pronounced with the aggravation of potassium deficiency, showing a similar trend to IAA and ABA. Yang et al. [34] believe that polyamines can stimulate plant growth and delay plant aging, while IAA can also promote cell division and accelerate plant growth. This indicates that polyamines may have a synergistic effect with IAA in the process of walnut seedlings responding to potassium deficiency stress [35]. Additionally, Zhang et al. [36] found that exogenous polyamines can reduce the level of reactive oxygen species (ROS) by enhancing the activity of antioxidant enzymes (SOD, CAT, and APX). Polyamines can also act as small molecular osmotic solutes to directly regulate osmosis, maintain cell turgor, and stabilize the structure and function of membranes [37]. It can be seen that polyamines such as Put, Spd, and Spm may play an important role as signaling molecules or metabolites in the physiological response process of walnut seedlings to potassium deficiency stress, and exogenous application of polyamines may promote the growth and tolerance of walnut seedlings under low potassium conditions and improve the utilization of potassium, but this requires further research.
Conclusions
This study suggests that walnut trees respond to potassium deficiency stress by producing large amounts of ABA. On the one hand, ABA regulates stomatal closure, reducing photosynthesis and transpiration to mitigate stress damage. On the other hand, as a signaling molecule, ABA modulates the changes in hormone levels such as IAA, CTK, and ethylene, as well as promotes the synthesis of polyamines. This collaborative effort accelerates cell division and improves potassium utilization, alleviating stress. Moreover, under short-term potassium deficiency stress, walnut seedlings can adjust their own metabolism, increasing investment in root development and enhancing respiratory activities to speed up the circulation of substances and energy within the plant, thereby enhancing their absorption capacity. However, under long-term potassium deficiency, the synthesis of various endogenous hormones and polyamines within walnut trees becomes disordered, leading to a significant weakening of photosynthesis, slow root growth, and ultimately affecting the entire plant’s growth, even causing rapid aging.

