

Introduction
The rapid development of intensive agriculture has brought about massively concentrated accumulations of organic waste, which has caused enormous pressure on the environment and resulted in the loss of useful nutrients [1, 2]. Pine forest accounts for 3.9% of the national forest area in China and covers about 21.06 million hectares of geographical area, with estimates of over 1.0 million tons of annual needle fall per thousand acres [3]. However, pine needles have become a challenging biomass from the perspective of harmless treatment due to the relatively high contents of silica and tannin.
Nowadays, aerobic composting has been accepted as a common method for resource utilization of organic solids from the perspective of both environmental friendliness and sustainable agriculture [4, 5]. It converts the macromolecular substances in organic waste and their auxiliary materials into carbon dioxide, ammonia, and high molecular weight humus through microbial aerobic fermentation. Based on the advantages, such as high fermentation temperature, short time required, and sufficient maturity of the final product as soil amendment [6], aerobic composting could be a suitable method for resource utilization of pine needles and poultry manure.
Generally, aerobic composting mainly consists of three stages, namely the mesophilic, thermophilic, and mature stages. During the thermophilic stage, the pile retains a high temperature, and microorganisms degrade the organic material and release a large amount of heat. Its efficiency determines the ripening process and thus impacts the mature quality of the end product. The application of immature high-phytotoxicity content compost products would result in water and soil pollution, especially for crop poisoning and root hazards due to the high content of phytotoxin [7]. In contrast, when compost is amended to soil, high-maturity composting products can be regarded as a source of organic nutrients for optimizing soil structural properties and fertility [8]. Therefore, how to accelerate composting maturity and produce superior quality compost has become a research hotspot. From this perspective, many researchers have utilized various methods to improve composting efficiency. They stated that using additives, such as jaggery and polyethylene glycol, reduces the composting process time and results in higher maturity composting [9]. However, according to their reports, the current additives are not cost-effective or efficient. Pine needles seem suitable for composting from the perspective of the environment and economy owing to their quality, high content of organic material, and huge quantity in China. Overall, the suitability of compost as a soil organic amendment depends on its chemical maturity and biological stability; therefore, the appropriate assessment of these parameters has great importance [10].
The main factors affecting composting efficiency are temperature, pH, C/N, moisture content, organic matter content, degree of compaction, etc. [11]. The starting material C/N has always been regarded as one of the most important variables influencing composting efficiency and product quality [12]. Generally, a starting C/N ratio of 25 to 35 is considered appropriate for aerobic composting. Low C/N can easily lead to the release of soluble salts and a large loss of nitrogen, resulting in reduced fertilizer efficiency [13]. Comparatively, higher C/N ratios will hamper the composting process by limiting microorganisms’ decomposition of organic materials, resulting in an extended fermentation cycle [14]. Therefore, regulating C/N has become an important method for controlling the composting process. However, although the influence of the C/N ratio is relatively well-characterized, the effect on the composting maturity involved in the succession of the activities of extracellular enzymes under different C/N ratios remains largely unexplored [15]. The driving force and its mechanism for high-efficiency composting through the secretion of extracellular enzymes using pig manure and pine needles as raw materials are supposed to furnish a strong theoretical model and basis for developing the organic fertilizer industry.
The high complexity of the organic materials demands the synergistic action of different extracellular enzymes (dehydrogenase, β-glucosidase, cellulase, protease, and phenoloxidase) to accomplish the composting degradation [16]. Dehydrogenase activity is considered a typical biological index that monitors the composting degradation process owing to its role in the respiratory chain [17]. In contrast, β-glucosidase, cellulase, phenoloxidase, and protease are associated with converting glycosides, cellulose, lignin, and N mineralization, respectively [18]. Thus, investigating the relationship between these enzyme activities and maturity succession will yield more information about controlling the composting process.
In an effort to understand the procession of the extracellular enzymes to different C/N ratios, aerobic composting with different C/N ratios based on different pine needle additions was performed. The composting process is monitored using representative key indicators that characterize composting maturity. The objectives of this research were to: 1) elucidate how the composting C/N ratio and stages impact the production of extracellular enzymes; 2) decipher specific key extracellular enzymes responsible for composting efficiency; and 3) infer the potential mechanisms related to organic material fermentation.
Materials and Methods
Compost Materials and Experimental Design
The aerobic composting was operated at the composting factory of Anhui Xinsheng Agricultural Industry Park Co., Ltd. (33°16′N, 116°19′E, 5.2 m a.s.l.) (Bozhou, China) using pine needle, pig manure, and mushroom residue as the initial substrates (Table 1). With different additions of pine needles, three composting types were established with three differing C/N ratios, namely pile 1 (C/N=15), pile 2 (C/N=25), and pile 3 (C/N=35) (Table 1).
Table 1.
Selected physicochemical characteristics of substrates used in composting construction (dry-weight based).
Prior to composting, the original materials were smashed into fragments with a length of less than 4 cm. The composting piles were mixed homogeneously using a tipping machine. The compost was subsequently arranged as a trapezoidal pile (2.6 m wide, 1.4 m high, and 5.0 m long). Subsequently, the starting moisture contents of the composting piles were adjusted to about 65%. To provide appropriate aeration, the composting piles were turned periodically (about every week) according to temperature variation by a mechanical composting turning methodology.
To achieve representativeness, samples were gathered at 0, 1, 6, 15, 27, and 36 days at three locations (the lower section: 10-15 cm; the middle section: 50-55 cm; the upper section: 100-115 cm). Then, each sample was subdivided into two parts: one part was stored at 4°C to detect enzymatic activities, and the second was air-dried and ground to 0.25 mm to determine key composting properties.
Measurement Methods
Ambient and composting temperatures were monitored at 10 a.m. every day by an automatic temperature measurement system uniformly inserted at four places in the composting piles. The pH value, concentrations of moisture, NH4+-N, NO3--N, water-soluble carbon (WSC), total carbon (TC), total nitrogen (TN), germination index (GI), and hemicellulose, cellulose, and lignin contents were quantified according to the methods described by Qiao et al. [12] with four replicates. For dehydrogenase activity, 1 g of fresh composting sample was dissolved in 2 ml of triphenyl-tetrazolium chloride and stored at 37℃ for 24 h away from light. After which, the suspension was filtered and colorimetric at 485 nm. Cellulase activity was quantified using 0.5% W/V carboxy methyl cellulose as a substrate buffer (pH 5.9) and then shaken, centrifuged, and concentrated. For β-Glycosidase, a 1.0 g fresh sample was suspended in 2 ml pNPG copyranoside, and then the release of p-nitrophenol was monitored spectrophotometrically at 410 nm. The 0.1 M Trise-HCl buffer (pH 8.1) and 2 mM benzyloxycarbonyl-phenylalanyl leucine buffer detected protease activity. The final detection of phenoloxidase was based on the oxidation of 2,7-diamino fluorenyldihydrochloride (2,7-DAF).
The Pot Experiment Design to Test the Promoting Growth Effect of the Composting Sample
To appropriately evaluate the growth-promoting effect of the composting end product, a pepper pot experiment was conducted in a greenhouse of a plant science park in Anhui Province, China, from February to May 2024. Three treatments were employed: pile 1, pile 2, and pile 3, corresponding to the end products of the pile 1, pile 2, and pile 3 treatments of aerobic composting, respectively. For each treatment, 4 replicate pots were performed, and thus, a total of 12 pots were achieved. Each pot was filled with 2.0 kg of soil, and 1.5% of ordinary organic fertilizer was added to the mix with the soil as the base fertilizer. Seedlings with uniform growth were selected for transplantation. After 42 days of transplantation, the plant growth parameters (stem diameter, plant height, and chlorophyll content (SPAD value)), and the aboveground fresh and dry biomasses of each treatment were measured.
Statistical Analysis
All statistical analyses were assigned a significance threshold of P < 0.05. Two-way analysis of variance (ANOVA) was conducted using PASW Statistics 22.0 (SPSS Inc., USA) to evaluate the influence of composting C/N ratios, stages, and their interactions on the typical enzymatic activities. Redundancy analysis (RDA) was applied using the “vegan” package in R (The R Foundation for Statistical Computing) to infer the association between enzymatic activities and physicochemical factors. Structural equation modeling (SEM) was carried out to evaluate the putative effects of enzymatic activities, the composting maturity, and selected physicochemical parameters using the DiagrammeR, dplyr, sem, vegan, and semPlot packages in R.
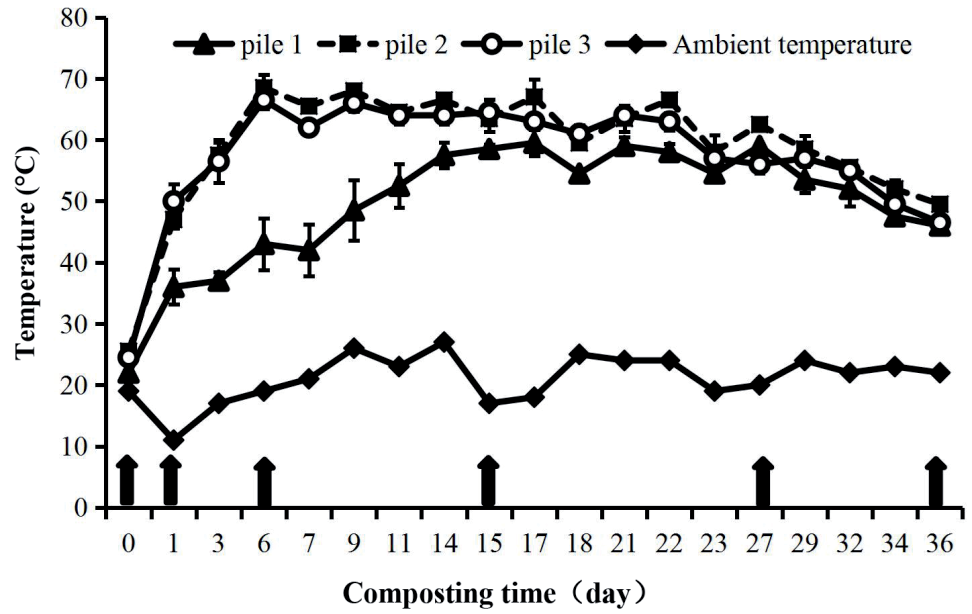
Fig. 1.
The variational temperatures (average mean temperatures of the top, middle, and bottom piles) of pile 1, pile 2, pile 3, and ambient during the aerobic composting. Arrows correspond to the days at which samples were collected: mesophilic (day 0, 1st), thermophilic (day 6th, 15th), and maturation (27th, 36th) composting stages. Values are the mean of three determinations, and bars represent the standard deviation.
Results and Discussion
Temperature Evolution
In the present study, the window temperature profiles at the composting factory complied with the general curve of the aerobic composting procedure, namely the mesophilic, thermophilic, and maturation stages (Fig. 1). Remarkably, piles 2 and 3 increased rapidly at the beginning of the process, reaching a maximum temperature of 67.5°C and 65.5°C on day 6, respectively, in comparison with pile 1, which peaked at 59.5°C on day 17. Simultaneously, piles 2 and 3 maintained thermophilic temperatures above 50.0°C for more consecutive days than pile 1. This higher temperature indicated that piles 2 and 3 accelerated the process of compost maturity [19]. At the end of the maturation stage, the temperature of all three treatments remained below 50°C.
Variations in Composting Parameters
The pH curves in the three piles indicated a consistent pattern of an initial increase followed by a gradual decline with the progression of composting (Fig. 2A). This was primarily due to the production of alkaline ammonia, the H+ release resulting from the microbial nitrification process, and low molecular organic acids, respectively [20]. The EC value of pile 1 indicated an increasing curve from 1.63 ms cm-1 to 3.06 ms cm-1 until day 25 and obtained higher values than piles 2 and 3 throughout the composting process (Fig. 2B). Here, the GI profiles for the three treatments revealed an anticipated increased trend until the maturation stage. Consequently, the appropriate C/N piles 2 (90.06%) and 3 (88.17%) indicated significantly higher GI in contrast to pile 1 (81.34%), suggesting a higher maturity of the compost with lower phytotoxicity [21]. Additionally, a declining trend for the C/N ratio was observed in the three piles as the decomposition progressed. When the composting ended, the C/N of the treatment piles 1, 2, and 3 were 13.35, 15.87, and 19.40, respectively. The final C/N ratio in all piles at values less than 20 confirmed compost maturity [22], exhibiting that the amendment of pine needles could regulate an approximate C/N ratio of 25-35 for high-efficiency composting. This result coincided well with previous reports by Xie et al. [23], who stated that initial compost C/N values between 25 and 40 were suitable for efficient composting.
As for the water-soluble components (Fig. 3), the NH4+-N contents rapidly increased to the maximum value on day 6 (6.26 mg g-1) in pile 1, as compared to pile 2 on day 6 (3.62 mg g-1) and pile 3 on day 1 (2.94 mg g-1), respectively. Thereafter, the NH4+-N contents of the three treatments indicated the same monotonous decreased patterns but at different speeds. Correspondingly, the NO3--N content in the three piles indicated a consistent increasing trend as the composting processed (P < 0.05). When the composting ended, the NO3--N content in pile 1 (71.92%) increased significantly higher than in pile 2 (56.91%) and pile 3 (55.48%). These variations are related to the sequence of material explanation during the composting process. In the early composting stage, easily degradable substances such as proteins and sugars were first humified. In the thermophilic and maturation stages, lignocellulosic substances began to degrade due to the high temperature [24]. Therefore, ammonium nitrogen increases in the early stage, while the nitrification reaction is strengthened in the later composting stage. Water-soluble carbon (WSC) contents in piles 1, 2, and 3 had an overall decreasing tendency and were reduced by 26.80%, 42.54%, and 36.19%, respectively, on day 36. This suggests that the degradation and incorporation of WSC by microbes was greater than the amount of newly synthesized soluble C [25, 26].
Fig. 2.
The evolution of selected maturity-related composting parameters. A: pH; B: EC; C: C/N ratio; D: Germination index (GI)
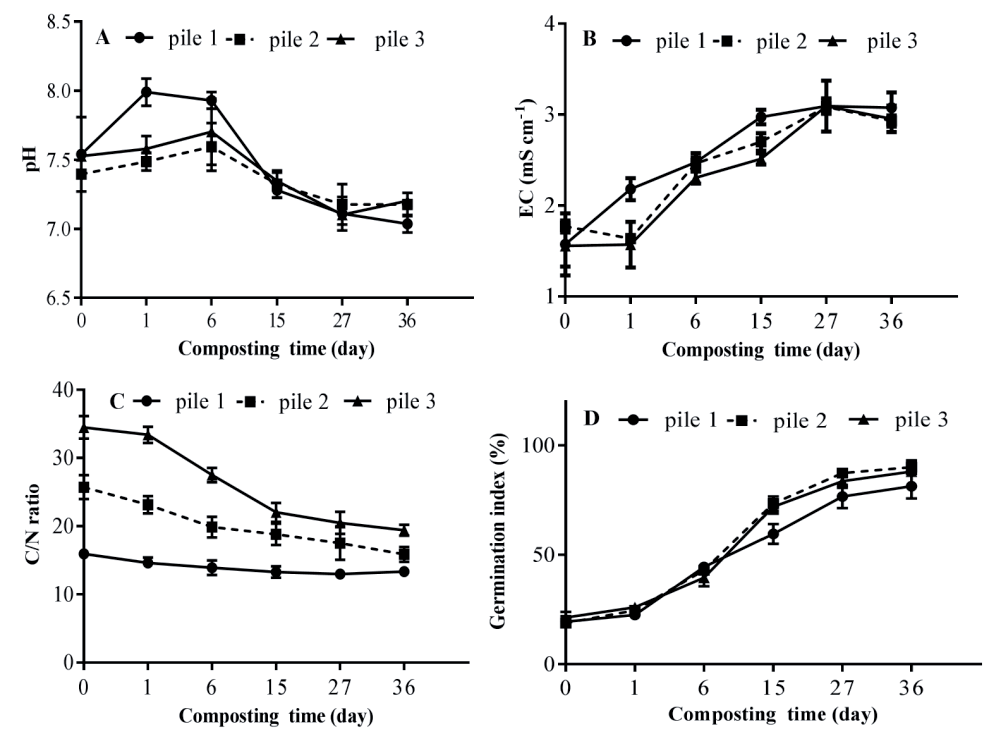
Fig. 3.
Dynamical variations of water-soluble carbon and nitrogen parameters. A: NO3 --N; B: NH4 +-N; C: NH4 +-N/NO3 --N; D: TOC
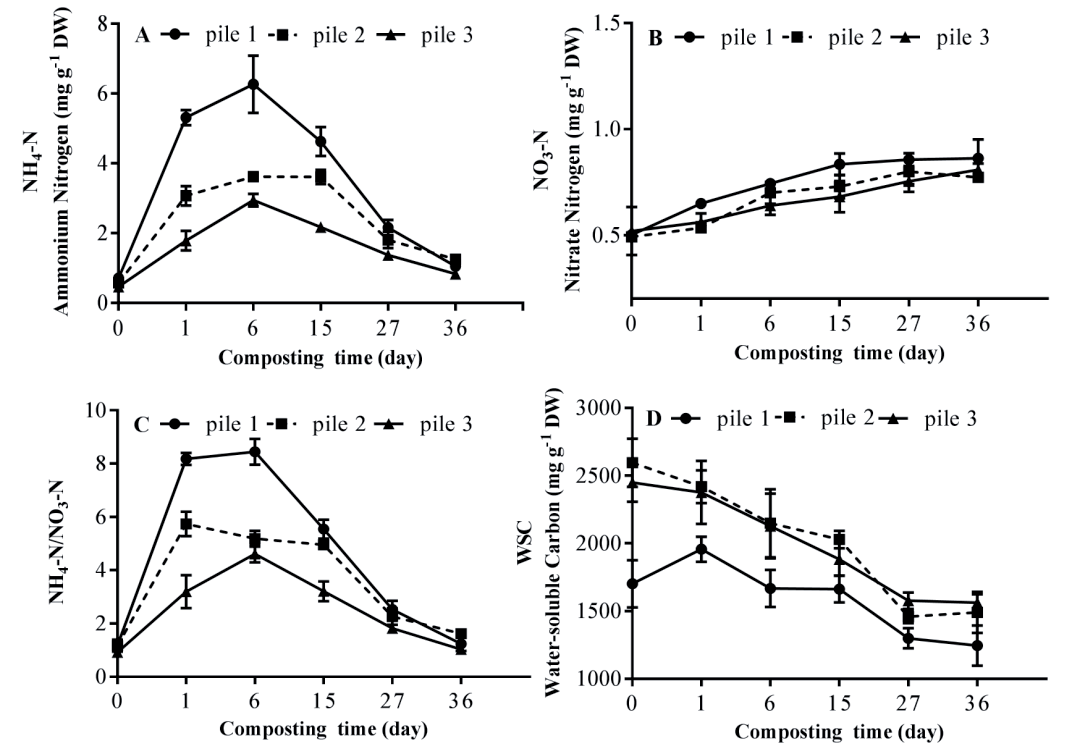
Fig. 4.
Dynamical variations of lignocelluloses parameters. A: Cellulose content; B: Hemicellulose content; C: Lignin content
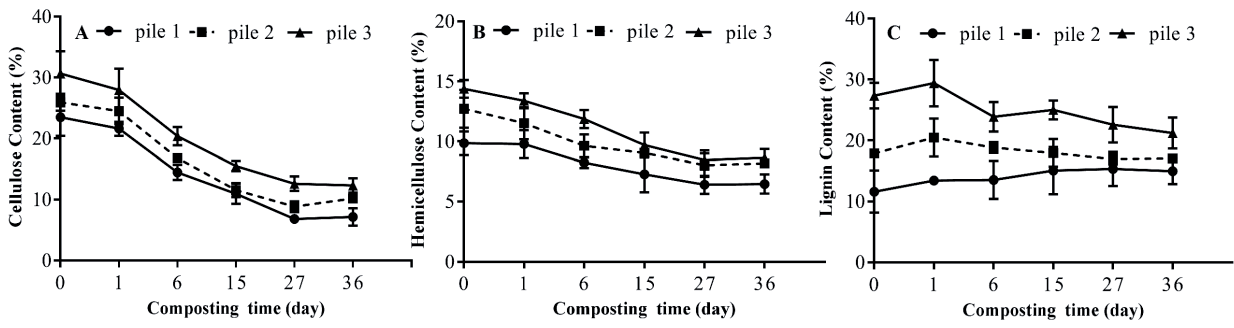
Overall, the cellulose and hemicellulose contents of the three treatments exhibited the same downward trend (Fig. 4). The cellulose content in pile 1 (69.49%) on day 36 was significantly higher than in piles 2 (60.71%) and 3 (59.77%), respectively, and hemicellulose indicated the same pattern. The degradation rate of lignin in pile 1 increased by 28.84%, whereas piles 2 and 3 declined by 4.61% and 22.38%, respectively, when the composting ended. Here, an increase in the lignin content was observed during the composting stages. Consequently, our results revealed speedy cellulose transformation during the thermophilic stage, and hemicellulose was basically stabilized from day 0 to day 27. The original contents of lignocellulosic compounds were highly variable due to the different composting compositions. Here, the lignin content showed a weak increase in the early composting process; similar results were found by Yang et al. (2021) [27], maybe due to the lower fermentation efficiency of the lignin fraction and the high degradation rate of other cellulosic components. As a result, piles 2 and 3 effectively accelerated the humification of lignocellulosic compounds and, therefore, accelerated the composting effectiveness. Adjusting C/N has become one of the important methods for controlling the composting process. The present study investigated the maturation process of aerobic composting with different ratios of pine needles in order to construct a high-temperature aerobic composting process with an optimal carbon-nitrogen ratio through pine needle amendment.
Variations in Enzymatic Analysis
The highest levels (974.56 U g-1) of dehydrogenase activity appeared in the early stages of the composting and then indicated a monotonically decreasing pattern until the composting ended. With respect to the composting treatment, significantly higher activities were harbored in piles 2 and 3 when compared to pile 1 (Table 2). The levels of β-glucanase activity peaked in the thermophilic stage (16.69 U g-1) and gradually decreased as the composting was processed. Regarding the composting treatment, piles 2 (14.94 U g-1) and 3 (15.85 U g-1) indicated significantly higher values than pile 1 (12.72 U g-1). As such, the evolution of cellulase activity exhibited the same pattern with β-glucosidase with the progression of the composting. Besides, the significantly higher levels of cellulase activity may be due to the higher lignocellulosic substances of pile 3 achieved by the addition of pine needles. It is generally accepted that protease could indicate the degradation of proteinaceous substrates involved in the nitrogen cycle [28]. Thus, higher levels of protease were present in pile 2, probably due to the higher concentration of polymeric macromolecules. Phenoloxidase functions on the lignin structure, and the complexity of the lignin structure also explains the differences and complementarities in the activities of these enzymes in this study [29]. Microorganisms transform organic substances in the composting pile by secreting extracellular enzymes; therefore, differences in enzyme activity lead to different degradation effects of substances.
Linking the Functional Enzymatic Activity with Environmental Parameters
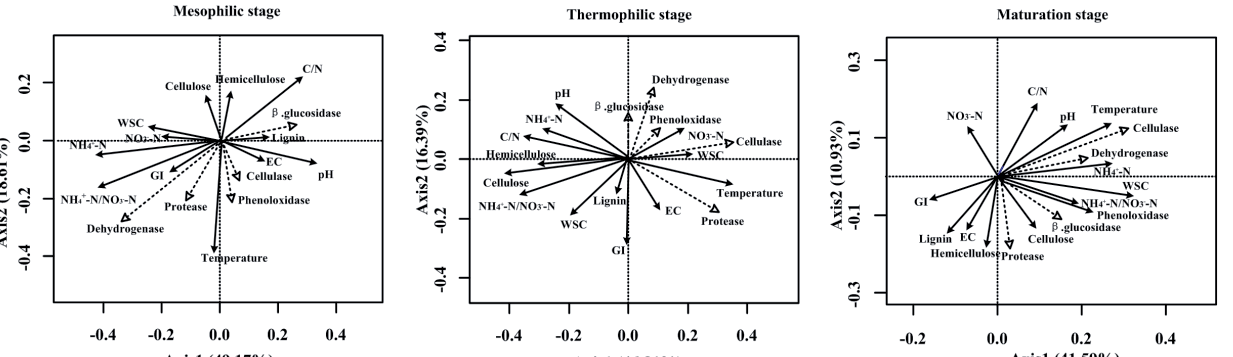
RDA was conducted to determine the associations between the investigated physicochemical properties and enzyme activities in the three stages (Fig. 5). A Monte Carlo permutation test indicated significant correlations in the mesophilic (Pseudo-F = 3.56, P < 0.01), thermophilic (Pseudo-F = 4.93, P < 0.01), and maturation stages (Pseudo-F = 4.51, P < 0.01), respectively. As illustrated by the arrow indication, of all the selected environmental factors, C/N ratio and temperature were the most related to the key extracellular enzymes. The temperature could impact the metabolization of the composting microorganisms, and C/N mainly plays a critical function in the readily available substrates to the microbial community [30]. Additionally, NH4+-N/NO3- -N, cellulose, and WSC were simultaneously confirmed as correlated to the dehydrogenase and β-glucosidase, protease, cellulase, and phenoloxidase activities in the mesophilic, thermophilic, and maturation stages, respectively. Remarkably, the first RDA component divided the composting piles and contributed 63.2% of the total variation in the thermophilic stage. Based on the previous discussion, the composting stages that were characterized by higher substrate bioavailability may be related to higher enzymatic activity. The observation of a significant correlation between composting maturity and cellulase activity showed the availability of cellulosic materials across the composting process [31]. Comparatively, β-glucosidase was observed to be significantly correlated with composting maturity in the mesophilic and mature stages. This was attributed to carbonaceous compounds derived from the cellulolytic and hemicellulolytic activities [32].
Table 2.
The enzymatic activities demonstrate a significant difference under different fertilizer treatments and stages.
Direct and Indirect Effects of Enzymatic Activity and Environmental Parameters on Composting Maturity
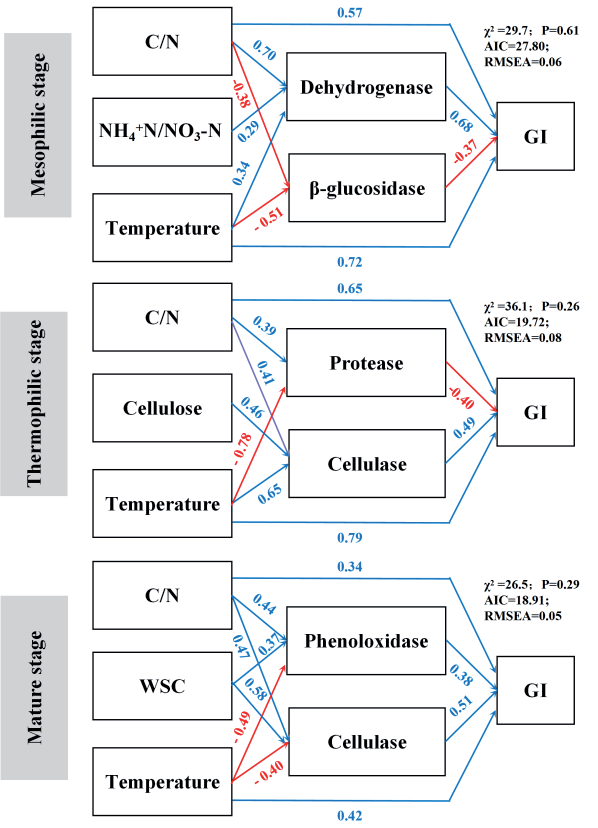
SEM analysis indicated that the composting microenvironment impacts the composting maturity by influencing the succession of enzymatic activity (Fig. 6). Overall, both the composting C/N and temperature indicated important positive and direct effects on the GI, followed by the cellulose, NH4+-N/NO3--N ratio, and WSC during the mesophilic, thermophilic, and maturation stages, respectively. Additionally, dehydrogenase (path coefficient = 0.63–0.79; P < 0.01) showed the highest positive and direct effects on the GI, followed by the β-glucosidase (0.24–0.49; P < 0.01) during the mesophilic stage. These results coincided well with previous reports based on cattle manure [33], which stated that enzymatic activity played a critical role in composting. When the composting was processed to the thermophilic stage, huge quantities of cellulose began to transform into water-soluble carbon, which regulated the GI value associated with cellulose activity (0.52–0.69; P < 0.01). The availability of readily metabolizable substrates, such as water-soluble carbon, influences enzyme synthesis, which establishes the balance between C and N, which accounts for the effects of nutrient availability on the composting maturity [34, 35].
Fig. 6.
Structural equation modeling illustrating the influences of C/N ratio on composting maturity by altering enzymatic activities. Numbers on arrows are equivalent to correlation coefficients; the arrow width indicates the strength of the causal relationship. The red arrows show positive relationships while the blue is negative, respectively.
Effects of the Composting End Product on the Growth of Plants
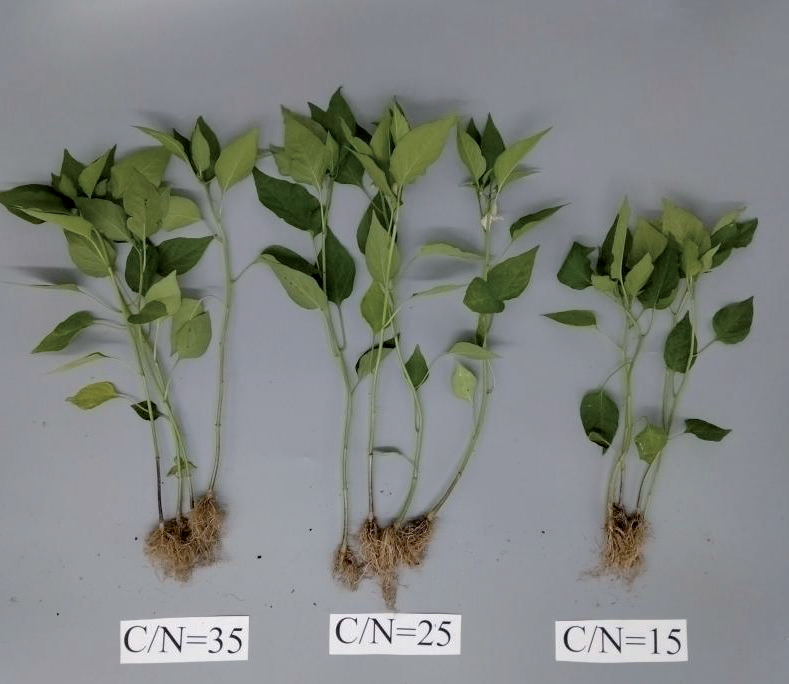
The composting products were used as culture media to determine the growth effects for pepper seedlings at this stage (Fig. 7). Stem diameter, height, SPAD, and fresh-dry biomasses were recorded 42 days after being planted in the pots (Table 3). At the end of the pot experiments, the plant heights of pile 2 were 79.01% and 18.03%, significantly higher than pile 1, respectively. Concurrently, the stem diameter, chlorophyll content, and fresh and dry biomasses of shoot values of pile 2 were also significantly higher than those of pile 1, but not the chlorophyll content and fresh biomass of shoots between piles 2 and 3. It is worth noting that the dry biomass of pile 2 was 72.73% and 14.46, significantly higher than pile 1 and pile 3, respectively. Overall, as the major determinants of seedling growth, these indexes indicated the plant growth-promoting of the aerobic composting end product of pile 2. This may be due to significantly better maturity, which provides more soluble nutrient availability and improves fertilizer efficiency [36]. Better maturity means it can break down organic matter into smaller molecules and increase the nutrient content to improve fertilizer utilization. Simultaneously, better maturity could mitigate the harmful substance content in fertilizers, thereby reducing crop harm [37]. In addition, composting can also improve soil structure, increase soil permeability, and increase water retention to achieve the plant growth-promoting effect [38]. Thus, the pot experiment with pepper seedlings proposed that the pile 2 treatment harbored significantly higher composting maturity, thus promoting growth.
Table 3.
Effects of applying the composting end product on heights, stem diameters, chlorophyll content, and fresh-dry biomasses of growing plants.
Conclusions
This study highlights the suitable C/N ratio of 25 to 35, which induced significantly higher efficiency aerobic composting, and the influence was attributed to the mechanisms such as: 1) the impact on the temporal variation of key physicochemical properties; 2) the selection and stimulation of functional extracellular enzymes such as protease, dehydrogenase, and cellulase; and 3) the expression and activity of enzymes potentially associated with key physicochemical properties. Overall, the initial composting C/N ratio induced the identified key functional enzymes and continuously adapted to the variational microenvironment, significantly contributing to composting efficiency. This study provides a theoretical basis and specific guidance for achieving efficient resource utilization of typical organic waste and large-scale industrial composting production.

