

Introduction
Medicinal plants are becoming increasingly significant for the economy due to the growing global trend of employing them to treat and improve human health [1, 2]. Salvia (Salvia sclarea L.), with approximately 900 species and a widespread distribution worldwide, holds great significance as the most prominent fragrant species within the Lamiaceae family and medicinal genus [3]. Salvia, also known as clary or clary sage, is a Mediterranean native herb highly valued in medicine, food, cosmetics, fragrance, and the pharmaceutical industry, and it has long been esteemed as one of the most effective medicinal plants [4]. This plant genus is known for its diverse biological properties, contributing to activating natural defense systems (antibacterial, antioxidant, anticancer, etc.) and stimulating anti-inflammatory-induced capacity [5]. The essential oil extracted from clary sage is experiencing high consumer demand, indicating significant market potential. The essential oil of clary sage contains important constituents such as geraniol, linalool, linalyl acetate, nerol, α-terpinyl acetate, and terpineol. These constituents may vary according to the growth stage and the specific part of the plant. Despite huge economic significance, the area under cultivation of clary sage has remained low in Asian and African countries, particularly in Egypt, owing to suboptimal yields and a lack of eco-friendly and pro-farmer plant nutrition management studies.
Among primary plant nutrients (nitrogen N, phosphorous P, and potassium K), N tends to trigger the vegetative growth of plants and determines the economic production of field crops [6]. The biosynthesis of plant components, critical for plant growth and the production of dry matter, relies heavily on N availability throughout the life cycle of crop plants [6]. However, N fertilizers have contributed significantly to greenhouse gas emissions from agricultural fields [7], along with concerns about the residue’s presence in the final product of medicinal plants. Previously, it was reported that N fertilizer (100 kg ha-1) remained effective in boosting the growth and essential oil yield of clary sage [8], while contrastingly, it was noted that clary sage growth and oil production and composition were enhanced with an N dose of 200 kg ha-1 [2]. Another study has reported that a low dose of N (3 g N plant-1) in comparison to higher N doses (4.5 and 6 g N plant-1) remained effective in boosting clary sage growth and essential oils productivity [9]. Thus, these contrasting findings necessitate reassessing N doses for boosting the yield and oil productivity of clary sage. Moreover, bio-organic farming has recently garnered significant attention to reduce reliance on agrochemicals, which have been associated with environmental pollution [10, 11].
Biofertilizers are organic compounds containing living microorganisms derived from farmland or root systems that promote plant growth through phytohormone production, leading to improved nutrient uptake as well as enhanced stress tolerance in plants without adversely affecting the environment or soil quality [2, 11, 12]. They play a significant role in atmospheric nitrogen fixation and phosphorus (P) solubilization [13-16]. Since utilizing cyanobacteria as biofertilizers can enhance soil fertility by enriching the soil with organic matter, cyanobacteria employed as biofertilizers can thereby promote plant growth and increase crop yield [17-19]. These trigger the biosynthesis of gibberellin, auxin, cytokinin [20-22], vitamins, amino acids, polypeptides, antibacterial and antifungal substances, and exopolysaccharides [17], which assist crop plants to survive abiotic stresses. The plant growth-promoting rhizobacteria (Bacillus subtilis or Pseudomonas fluorescens or Cyanobacteria or Trichoderma) enhanced the nutrient content of clary sage [23]. The biological nitrogen fixation (BNF) processes increased N and P availability in the soil, which led to significantly higher growth of the crop plants [24]. Additionally, it has been demonstrated that the accelerated mineralization rate of soil organic residues leads to an increase in soil carbon (C) and sulfur (S) contents following inoculation with Azotobacter species [25]. These can directly increase plant growth by producing plant growth hormones like indole acetic acid (IAA), gibberellins, and cytokinin, as well as by improving nutrient uptake [26, 27].
The most thoroughly studied genus of heterotrophic, free-living, N2-fixing bacteria is Azotobacter. The abundant synthesis of exopolysaccharides (EPS) by Azotobacter has been reported previously [28]. It utilizes atmospheric N gas to synthesize cell proteins, and upon their death, these proteins are mineralized in the soil, releasing plant-available N. It acts as plant growth-promoting rhizobacteria, having unmatched potential to produce biologically active compounds such as IAA, gibberellins, and B vitamins in culture conditions for enhanced atmospheric N fixation [29]. Azotobacter chroococcum is a heterotrophic, symbiotic N fixer that can fix an average of 20 kg N ha-1 annually [25]. Azotobacter speeds up the mineralization of organic waste in the soil, thereby making nutrients (N, P, and S) available for crop plants. Additionally, it aids in the absorption of macro and certain micronutrients, improving the plant’s ability to use its root exudates [30]. Azotobacter strains improved growth and productivity, and in particular, N availability was required in abundance to promote the vegetative growth of cereal and pulse crops [31-33]. Therefore, it is of vital interest to assess its effectiveness for clary sage.
Blue-green algae (BGA) are also referred to as cyanobacteria, especially in the context of discussing organisms in water that produce their own food. However, cyanobacteria are not taxonomically related to other organisms classified as algae. In N-deficient situations, cyanobacteria can use nitrogenase enzymes to fix atmospheric N2 into plant-available ammonium [34]. Therefore, cyanobacteria have remained effective in increasing the N compounds in paddy fields and improving the physical and chemical characteristics of soil by excreting chemicals that promote growth [35, 36]. Due to its natural growth and widespread availability, aloe vera is a perennial plant that thrives well in temperate and sub-temperate climates, along with offering high nutritional value at a low cost [37]. However, to the best of our literature search, there exist knowledge and research gaps pertaining to the appropriate N doses and the most suitable NFB species for promoting the growth and oil concentration of clary sage in Egypt, which necessitates conducting further field studies.
Therefore, the current study examined the effects of mineral N fertilizers and biological fertilizers (Azotobacter chroococcum and Cyanobacteria) on concentrations of macro- and micro-nutrients, nitrogenase and dehydrogenase activities in the rhizosphere, fluorescence (Fv/Fm), pigment status measured by SPAD-value, normalized difference vegetation index (NDVI), leaf area, dry matter production, oil content, and the main essential oil composition of Salvia sclarea. The ultimate aim was to sort out the most performing N dose and biofertilizer in terms of clary sage growth, nutrient uptake, and essential oils composition to boost its cultivation and quality in Egypt.
Materials and Methods
Preparation of Plant-Based Culture Media (Aloe Vera)
Succulent leaves of aloe vera were meticulously cleansed and then blended with equal volumes of distilled water (w/v) for 5 minutes by using a blender. The resultant slurry homogenate underwent a coarse filtration process through cheesecloth to yield plant juice, with approximately 73–82% of the plant’s original fresh weight being recovered in the form of liquid. The extracted plant juices from the specimens under scrutiny were subsequently subjected to further dilution with distilled water (v/v) at varying ratios of 1:10, 1:20, 1:40, 1:80, and 1:100. The pH range of the diluted aloe vera juice was measured between 4 and 6.2. These diluted juices were harnessed exclusively to formulate the plant-based agar culture medium containing 2% agar (w/v). The pH of the culture medium was meticulously adjusted to 7.0 using calcium carbonate prior to undergoing autoclaving at 1.5 atm and 121 °C for 20 minutes. The isolation of rhizosphere microorganisms was conducted through a series of dilutions. A rhizosphere soil sample of 1.0 g was introduced into 10 ml of sterile distilled water under stringent aseptic conditions. This mixture was agitated vigorously for 10 minutes using a vortex set at 150 rpm and allowed to settle briefly. A sequential set of serial dilutions was performed, starting from the stock solution and progressively diluted down to 10-6. From each dilution tube, 0.1 ml of the suspension was carefully transferred onto the surface of the plant-based agar media incorporated with aloe vera (performed in triplicate). Subsequently, the suspension was evenly spread using an alcohol-sterilized L-shaped glass rod. The prepared agar plates were incubated at 30 °C for 24 to 48 hrs. After successfully cultivating microorganisms, individual colonies were meticulously isolated and purified for further study [37].
Field Experiment
A field experiment was carried out at the Agricultural Experiments and Research Station at the Faculty of Agriculture, Cairo University, Giza, Egypt, during 2019-20. The site is located at 30°01′38′′ N latitude and 31°11′35′′ E longitude.
Germany’s Jelitto seed company provided the seeds of clary sage. After being sterilized with sodium hypochlorite solution (10%) for 15 minutes, seeds of the same size and color were rewashed in distilled water and then air dried. Seeds were sown in plastic pots (23 x 18 cm) containing a 1:1 ratio of sand and clay soil on 26 December 2019. The seedlings were moved into the open field on 26 February 2020. Clary sage was planted at a density of 14,500 plants per hectare in experimental units having an area of 5.5 × 4.5 m each and R×R spacing of 50 cm. Before sowing, the experimental field was plowed. The experimental soil was loamy clay, having 6% coarse sand, 33.1% fine sand, 40.2% silt, and 25.1% clay. Its physicochemical properties included 7.3 pH and 1.85% organic matter, along with available N, P, and K concentrations of 7.3, 6.4, and 160 mg kg-1, respectively. Superphosphate (15.5% P2O5) fertilizer (32 kg P ha-1) was applied as a basal dose during the final land preparation. However, potassium was added (95 kg K ha-1) in two equal doses, the first added as a basal dose and the second dose added 30 days after transplanting (DAT). All other cultural practices were performed following the recommendation of the Ministry of Agriculture and Land Reclamation, Egypt.
The experiment was conducted in a split-plot layout in a randomized complete block design (RCBD) with three replications. Two main plots were assigned to one mineral N fertilizer in each replication. Each main plot was divided into four sub-plots, wherein three sub-plots were inoculated with Azotobacter or Cyanobacteria or Azotobacter + Cyanobacteria bio-fertilizer, and the rest one was assigned as control (untreated). Two levels of N fertilizers, viz., 50% and 100% of the recommended dose (120 kg N ha−1) of ammonium sulfate (20.5% N), were used. Therefore, a total of eight treatment combinations of two factors (N fertilizers and nitrogen-fixing bacteria, NFB), viz., T1 = 120 kg N ha−1 without NFB, T2 = 120 kg N ha−1 + Azotobacter, T3 = 120 kg N ha−1 + Cyanobacteria, T4 = 120 kg N ha−1 + Azotobacter + Cyanobacteria, T5 = 60 kg N ha−1 without NFB, T6 = 60 kg N ha−1 + Azotobacter, T7 = 60 kg N ha−1 + Cyanobacteria, and T8 = 60 kg N ha−1 + Azotobacter + Cyanobacteria were assessed in the study. The culture media of aloe vera was used as the growth media for the studied bacteria. The media culture contained 108 cfu/ ml of bacteria and was supplied with irrigation, and the crop was harvested at 130 DAT.
Data Collection
Plant Growth Traits, Normalized Difference Vegetation Index (NDVI), Chlorophyll Fluorescence (Fv/ Fm), and Chlorophyll Content (SPAD Value)
Ten randomly selected plants from each plot were evaluated at 120 DAT for growth parameters, such as the leaf area (LA) per plant and the shoot dry weight (SDW) per plant. The LA per plant was measured using a leaf area meter (LiCOR 3100; Licor, Lincoln, NB, USA), while the SDW per plant was determined after oven-drying the samples at 70 °C for 48 hrs.
The NDVI was estimated with a field-portable NDVI sensor (Green Seeker® Handheld Crop Sensor, Trimble Navigation Limited, Westminster, CO, USA). Following transplantation, measurements were taken on each plot 120 days later. The sensor head was fixed 60-120 cm horizontally over the crop in the middle row of the plot.
The Fv/Fm was measured at 120 days after transplantation (DAT) for five plants from each treatment by using a portable fluorometer (Handy PEA, Hansatech Instruments Ltd., Kings Lynn, U.K.).
The SPAD readings were recorded using a SPAD-502 Plus meter (Konica Minolta, Inc., Japan). The SPAD- 502 Plus meter detects the transmittance of red (60 nm) and infrared light (940 nm) to determine the amount of chlorophyll. Two LEDs (light-emitting diodes) with peak wavelengths of 650 and 940 nm produce light. Twelve independent SPAD measurements were made with different plants on each plot.
Macro and Micronutrients
The shoot samples were dried at 70 °C in an electric oven for 72 hrs. At 120 DAT, the dried branches were sampled to determine the concentrations of the macronutrients such as N, P, K+, calcium (Ca2+), and magnesium (Mg2+), as well as the micronutrients such as boron (B), zinc (Zn2+), manganese (Mn2+), iron (Fe3+), and copper (Cu2+). Total N content was determined by using the micro-Kjeldahl method. The P content was determined colorimetrically/Zarrouk, 1966 #37// by using a stannous chloride-ammonium molybdate reagent after extraction by sodium bicarbonate [38]. The K content was measured using a flame photometer (ELE Flame Photometer, Leighton Buzzard, UK). Other nutrients like Ca2+, Mg2+, Fe3+, Mn2+, Zn2+, and Cu2+ concentrations were measured by atomic absorption spectrophotometry [55]. N, P, K+, Ca2+, and Mg2+ were expressed as grams per kilogram, g kg−1, while Fe3+, Mn2+, Zn2+, and Cu2+ were expressed as mg kg−1.
Essential Oil Yield, Nitrogenase Measurements, and Dehydrogenase Activity Measurements
To determine the fresh weight (FW), plants were harvested 10 cm above the plant’s neck to avoid mechanical damage and promptly weighed. The essential oil content (mL kg-1 DW: dry weight) was measured from four randomized subsamples of 125 g of vegetal material (500 g) in each treatment following the method described by [39]. Nitrogenase activity was assessed in plant samples collected at 120 DAT. Acetyl reduction was used to measure the enzyme activity [40]. The dehydrogenase activity (DHA) was assessed at 120 DAT. The DHA was estimated using triphenyltrterazolium chloride (TTC) as a synthetic electron acceptor [41].
Statistical Analysis
Data were subjected to analysis of variance (ANOVA) using a split-plot design [42]. The Levene and Shapiro-Wilk tests were used to detect the homogeneity of the error variances and normal distribution [43, 44]. The statistically significant differences between means at p ≤ 0.05 were determined using the Tukey HSD (honestly significant difference) multi-comparison test. The statistical analysis was employed using GenStat 19th Edition (VSN International Ltd, Hemel Hempstead, UK).
Results
Growth Curve of Azotobacter and Cyanobacteria on Natural and Synthetic Medium
Azotobacter chroococcum growth on natural and synthetic media showed the maximum increase of 0.915nn and 0.871nn at three days of synthetic media and natural media, respectively, as shown in Table 1. Data in Table 2 showed that the Nostoc muscorum achieved the highest biomass of 0.47 mg DW L-1 medium, while the Anabaena fertilissima exhibited biomass of 0.57 mg DW L-1 medium after three weeks, both in synthetic medium. After the same period (3 weeks), the highest biomass values were 0.45 mg DW L-1 medium for Nostoc muscorum and 0.51 DW L-1 medium for Anabaena fertilissima, both in natural media.
Table 1.
Azotobacter chroococcum bacteria growth curve on natural and synthetic medium.
| Day | O.D 600nn | |
|---|---|---|
| Azotobacter chroococcum | ||
| Natural media | Synthetic media | |
| 1 | 0.27 | 0.45 |
| 2 | 0.59 | 0.78 |
| 3 | 0.87 | 0.91 |
| 4 | 0.86 | 0.91 |
| 5 | 0.85 | 0.85 |
| 6 | 0.63 | 0.79 |
Table 2.
Cyanobacteria strains biomass grown on natural and synthetic media at different periods.
Nitrogenase Activity
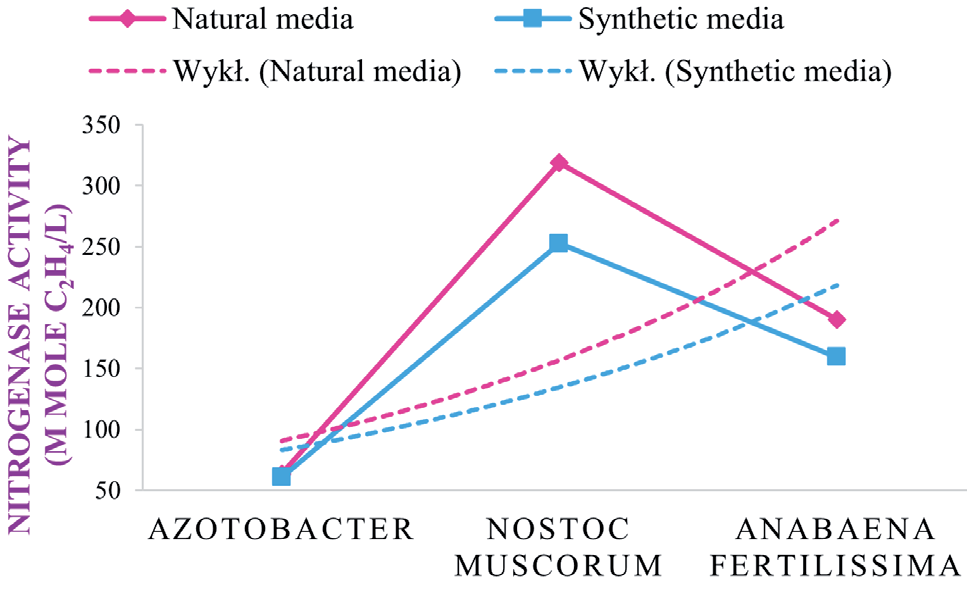
The nitrogenase activity values of bacterial strains (Azotobacter, Nostoc muscorum, and Anabaena fertilissima) exhibited the highest nitrogenase activity, with values of 63.60, 318.64, and 190.17 µ mole C2H4/L, respectively, when grown on a natural medium (Fig. 1). These values surpassed the nitrogenase activity observed when the same strains were cultivated on synthetic media.
Rhizosphere Enzymes under N Deficiency
When the recommended N fertilizer rate of 120 kg N ha−1 was applied, as opposed to 60 kg N ha−1, it resulted in a significant increase in dehydrogenase and a considerable decrease in nitrogenase activity in clary sage plants (Fig. 2). The inoculation of clary plants with Azotobacter or Cyanobacteria or Azotobacter + Cyanobacteria significantly increased the nitrogenase and dehydrogenase activity over control. Plant inoculation with the combination of Azotobacter and Cyanobacteria recorded the highest values of nitrogenase and dehydrogenase activity compared to all other studied treatments. The co-application of Azotobacter and Cyanobacteria resulted in a remarkable increase in nitrogenase activity by 172.8% and dehydrogenase activity by 47.6% compared to the control plants. The interaction effects were significant for nitrogenase and dehydrogenase activities, and remarkably, we noticed that the application of 60 kg N ha−1 plus Azotobacter + Cyanobacteria gave the highest values for nitrogenase and dehydrogenase activities. Application of only 60 kg N ha−1 plus Azotobacter + Cyanobacteria compared to 120 kg N ha−1 without using NFB resulted in a significant increase in nitrogenase activity, which was 210% (Fig. 2).
Plant Nutrients under N Deficiency
The main effect of the application of the recommended N fertilizer rate at 120 kg N ha−1 compared to 60 kg N ha−1 increased N, P, K, Ca, Mg, B, Zn, Mn, Fe, and Cu contents in clary sage plants (Table 3). The inoculation of clary plants with Azotobacter or Cyanobacteria or Azotobacter + Cyanobacteria increased the nutrients over untreated plants. The highest concentration of N, P, K, Ca, Mg, B, Zn, Mn, Fe, and Cu was observed when the plants were inoculated with the combination of Azotobacter and Cyanobacteria compared to the rest of the treatments. Application of Azotobacter + Cyanobacteria increased the N, P, K, Ca, Mg, B, Zn, Mn, Fe, and Cu by 31.7, 12.7, 9.1, 24.8, 43.0, 25.8, 5.4, 4.4, 4.2, and 10.3%, respectively, compared to untreated control plants (Table 3). Interaction effects were significant in all mentioned traits, and it was noticed that the application of 120 kg N ha−1 plus Azotobacter + Cyanobacteria gave the highest concentration for all nutrients. It was recorded that 60 kg N ha−1 plus Azotobacter + Cyanobacteria remained superior to the 120 kg N ha−1 without using NFB by recording the significant increase of N, P, Mg, Mn, and B accounted for by 8.0, 3.9, 25.1, 1.3, and 2.2%, respectively (Table 3).
Fig. 2.
Effect of N-fixing bacteria and fertilization on the nitrogenase activity (nmol C2H4 g/dry soil/hr) and denitrogenase activity in the soil rhizosphere of clary sage plants. T1: 120 kg N ha−1 without NFB, T2: 120 kg N ha−1 + Azotobacter, T3: 120 kg N ha−1 + Cyanobacteria, T4: 120 kg N ha−1 + Azotobacter + Cyanobacteria, T5: 60 kg N ha−1 without NFB, T6: 60 kg N ha−1 + Azotobacter, T7: 60 kg N ha−1 + Cyanobacteria, and T8: 60 kg N ha−1 + Azotobacter + Cyanobacteria.
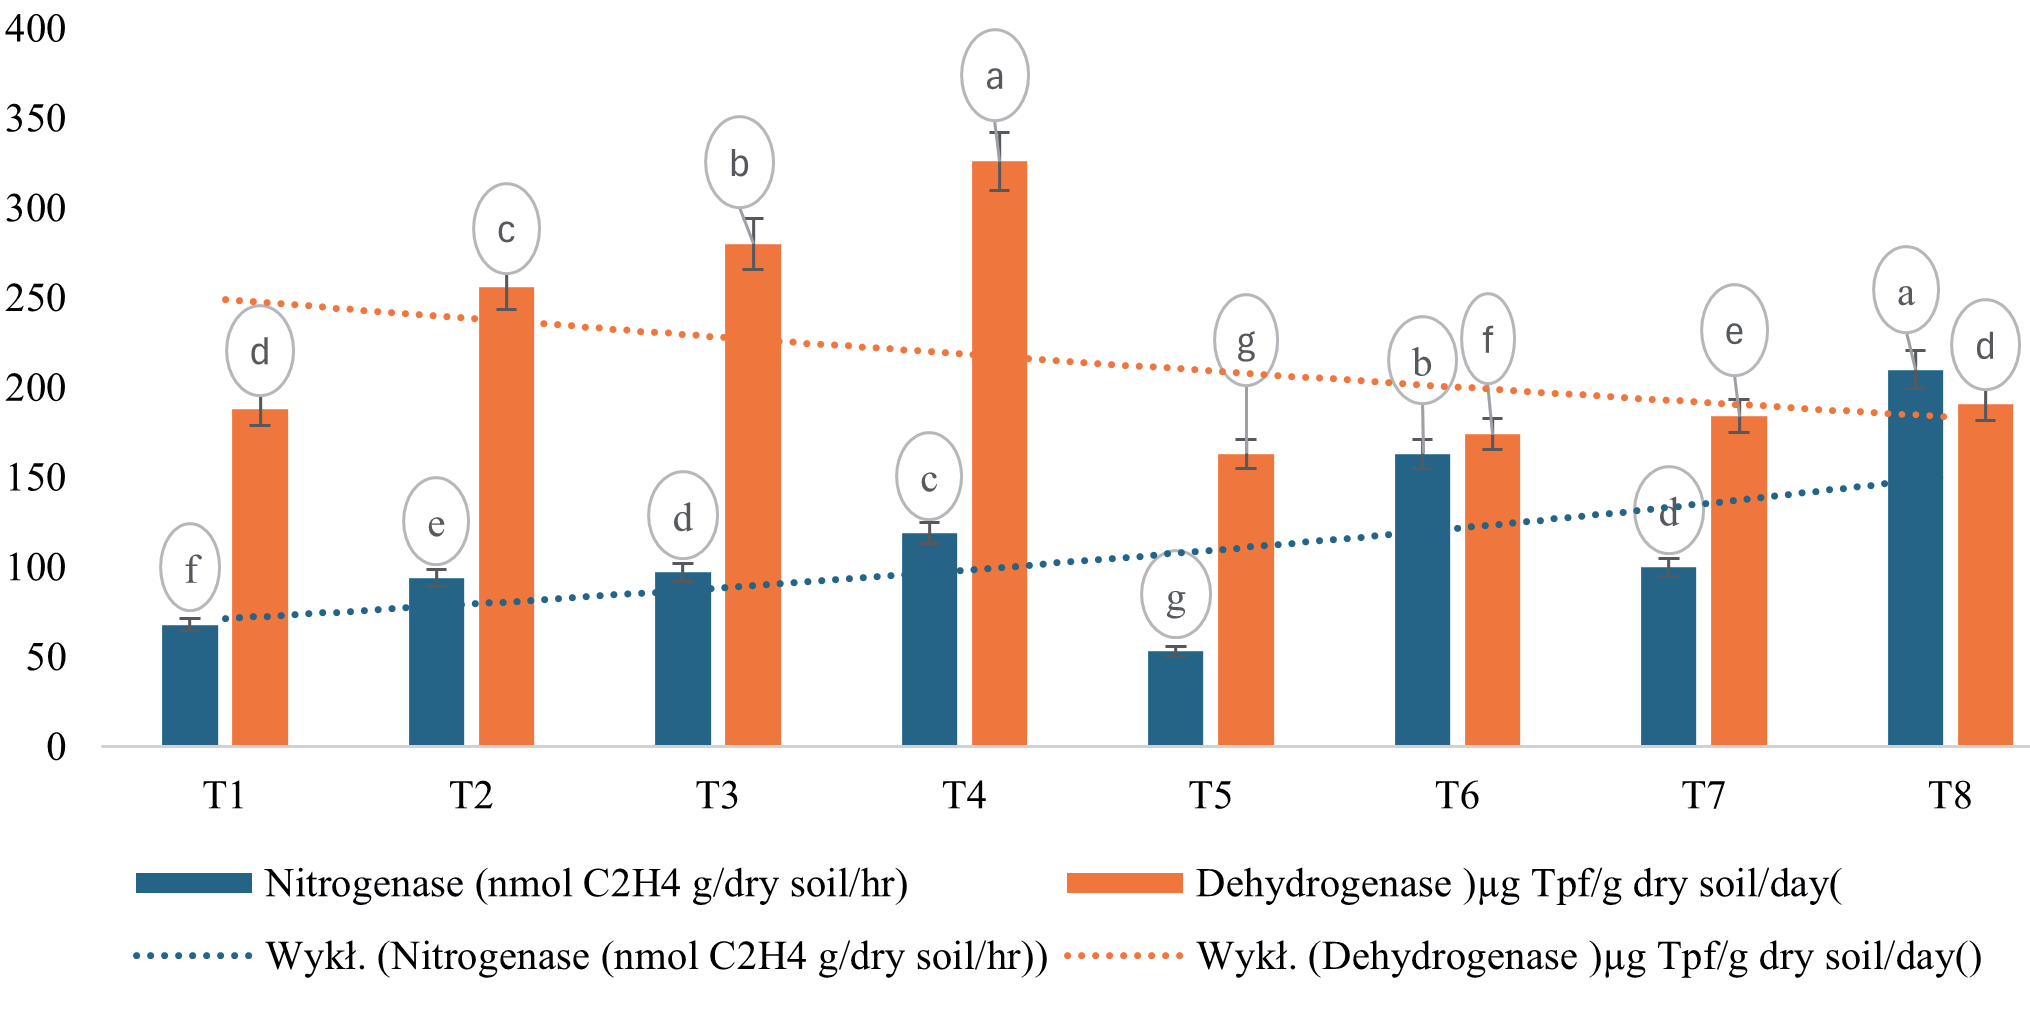
Table 3.
The impact of N-fixing bacteria and N fertilization on the concentrations of macro-nutrients (N, P, K, Ca, Mg) and micronutrients (B, Zn, Mn, Fe, Cu) of Clary sage plants.
[i] Note: †Data followed by the same letter in a column are not significantly different according to ’Tukey’s honestly significant difference (HSD) test at P ≤ 0.05, NFB: Nitrogen fixing bacteria, T1: 120 kg N ha−1 without NFB, T2: 120 kg N ha−1 + Azotobacter, T3: 120 kg N ha−1 + Cyanobacteria, T4: 120 kg N ha−1 + Azotobacter + Cyanobacteria, T5: 60 kg N ha−1 without NFB, T6: 60 kg N ha−1 + Azotobacter, T7: 60 kg N ha−1 + Cyanobacteria, and T8: 60 kg N ha−1 + Azotobacter + Cyanobacteria.
Physiological Response under N Deficiency
Applying 120 kg N ha−1 compared to 60 kg N ha−1 significantly increased the Fv/Fm, SPAD-value, and NDVI (Table 4). Inoculation of Azotobacter or Cyanobacteria or Azotobacter + Cyanobacteria in clary plants significantly improved the values of Fv/ Fm, SPAD-value, and NDVI as compared to control plants. The highest values of Fv/Fm, SPAD-value, and NDVI were recorded in plants when inoculated with Azotobacter and Cyanobacteria as compared to the control. The combination of Azotobacter and Cyanobacteria increased the Fv/Fm, SPAD-value, and NDVI by 6.7%, 19.1%, and 9.3%, respectively (Table 4). Significant interaction effects were observed across all mentioned traits, and it was noted that the application of 120 kg N ha−1 plus Azotobacter + Cyanobacteria yielded the highest concentration of all the mentioned nutrients. However, the application of only 60 kg N ha−1 plus Azotobacter + Cyanobacteria compared to 120 kg N ha−1 without using NFB resulted in a significant increase in Fv/Fm, SPAD-value, and NDVI of 2.7, 11.1, and 1.7%, respectively (Table 4).
Growth Response under N Deficiency
Applying 120 kg N ha−1, compared to 60 kg N ha−1, resulted in a significant increase in the leaf area (LA) and dry weight (SDW) of the clary sage plants (Table 4). Inoculation of Azotobacter or Cyanobacteria or Azotobacter + Cyanobacteria in plants considerably increased the LA and SDW as compared to control. Meanwhile, the inoculation of Azotobacter + Cyanobacteria showed the highest values of LA and SDW in clary plants compared to other treatments. Compared to untreated control plants, the integration of Azotobacter + Cyanobacteria increased the LA and SDW by 46.2% and 54.4%, respectively (Table 4). Interaction effects were significant in all mentioned traits, and the application of 120 kg N ha−1 plus Azotobacter + Cyanobacteria gave the highest concentration for all the above-mentioned nutrients. Nevertheless, applying only 60 kg N ha−1 plus Azotobacter + Cyanobacteria compared to 120 kg N ha−1 without using NFB led to a significant increase in both LA and SDW by 23.1 and 21.6%, respectively (Table 4).
Table 4.
The effects of N-fixing bacteria and N fertilization on the quantum efficiency of PSII in dark-adapted conditions (Fv/Fm), SPADvalue, NDVI, leaf area, and dry weight of Clary sage plants grown under two N fertilizer rates.
[i] Note: †Data followed by the same letter in a column are not significantly different according to ’Tukey’s honestly significant difference (HSD) test at P ≤ 0.05, NFB: Nitrogen fixing bacteria, T1: 120 kg N ha−1 without NFB, T2: 120 kg N ha−1 + Azotobacter, T3: 120 kg N ha−1 + Cyanobacteria, T4: 120 kg N ha−1 + Azotobacter + Cyanobacteria, T5: 60 kg N ha−1 without NFB, T6: 60 kg N ha−1 + Azotobacter, T7: 60 kg N ha−1 + Cyanobacteria, and T8: 60 kg N ha−1 + Azotobacter + Cyanobacteria.
Essential Oil Constituents under N Deficiency
The recommended N fertilizer rate at 120 kg N ha−1, compared to 60 kg N ha−1, resulted in a significant increase in oil percentage, α-pirena, camphene, B-prnene, limonene, linalool, camphor, terpineol, bomeal, bonnylacetate, eugenol, and β-caryophyllene. (Table 5). The integration of clary sage plants with Azotobacter or Cyanobacteria or Azotobacter + Cyanobacteria caused a significant increase in oil %, α-pirena, camphene, β-prnene, limonene, linalool, camphor, terpineol, bomeal, bonnylacetate, eugenol, and β-caryophyllene as compared to untreated plants. The application of Azotobacter and Cyanobacteria increased the oil percentage by 52.8% compared to untreated control plants. Significant interaction effects were observed in all the mentioned traits. However, it was observed that the application of 60 kg N ha−1 in combination with Azotobacter and Cyanobacteria improved these traits compared to using 60 kg N ha−1 without using NFB (Table 5).
Correlation Matrix Analysis of Response Variables
A correlation matrix analysis was conducted to determine the nature and degree of association (correlation coefficients of 0.9-1.0 are highly significant, 0.5-.09 are significant, 0.1-0.5 are weak, and 0-0.1 are uncorrelated, whereas the ‘–’ symbol indicates the negative or inverse association between two variables) among different response variables of clary sage (Table 6). The results indicated that nitrogenese was negatively associated with DHA (-0.037**), Fe (-0.017**), and Zn (-0.235**) content, while it had a positive relationship with the rest of the response variables. In addition, macronutrients (N, P, and K) were recorded to have positive associations with micronutrients (Ca, Mg, Mn, Zn, Fe, B, and Cu) and other response variables (NDVI, LA, SFW, etc.). Among micronutrients, Zn recorded a negative association with nitrogenese activity, while other associations were significantly positive. Moreover, the vegetative growth traits demonstrated a significantly positive association with the response variables, and no negative correlation was detected. Likewise, the leaf area depicted an incredibly strong association with the Mg (0.992**), Fv/Fm (0.929**), SPAD (0.968**), and the NDVI (0.941**) values; however, it had a weak relationship with the nitrogenese activity (0.437*). Likewise, the SDW of clary sage exhibited a strong relationship with macronutrients (N, P, and K) as well as the Fv/Fm, SPAD, and NDVI values. Interestingly, the essential oil was recorded to have a strong association with the DHA, P, K, Cu, Fv/Fm, and NDVI, whereas it exhibited a weak association with the nitrogenese activity.
Discussion
In this study, an alternative natural media was prepared using aloe vera plants, aimed at mitigating the excessive costs associated with synthetic growth media. This plant has been known for its richness in various compounds such as salicylic acid, amino acids, lignin, saponins, carbohydrates, vitamins, enzymes, minerals, and sugars. Additionally, it is abundant in antioxidant vitamins A, C, and E, as well as folic acid and vitamin B-12 [45]. Such natural media could serve as a culture medium for rhizobacteria that enhances plant growth. Synthetic media have become more valuable than natural media, especially when considering the optical density (OD) of Azotobacter chroococcum. On the contrary, azotobacter chroococcum and cyanobacteria (Anabaena fertilissima and Nostoc muscorum) showed higher nitrogenase activity in natural media than in synthetic media [45].
Given the significant role that enzymes play in nutrient cycles, the enzymatic activity of soil samples serves as a vital indicator of soil fertility [46, 47]. The enzymatic activities in the rhizosphere of the clary sage plant, whereas the rates of mineral N fertilizer, had an impact on the DHA in soil in this study. The highest level of DHA was observed when organic Azotobacter chroococcum was treated with the indicated rate of mineral N. This could be attributed to the enhanced rate of N2 fixation by Azotobacter chroococcum, which likely played a significant role in stimulating plant growth in the rhizosphere [48, 49]. This could lead to the accumulation of nutrients and the stimulation of soil rhizosphere bacteria, thereby promoting plant growth and overall soil health. It was observed that the nitrogenase activity was increased by inoculation with either cyanobacteria or azotobacter chroococcum. The interaction treatments involving reduced N rate with all biofertilizer treatments yielded the greatest mean values for the nitrogenase enzyme. Like our findings, it was reported that inoculating with N-fixing bacteria positively impacted the nitrogenase activity [50].
The soil under a study with Salvia spp. exhibited greater availability of nutrients after the application of mineral N fertilizer and biofertilizer. Consequently, applying mineral N fertilizer and biofertilizer significantly increased the nutrient content of Salvia spp. [51]. Those results agree with our findings, where the application of cyanobacteria or Azotobacter + Cyanobacteria led to increased concentrations of macronutrients (N, P, K, Ca, Mg) and micronutrients (B, Zn, Mn, Fe, Cu) in sage plants. These results could be attributed to the release of applied nutrients into the soil solution and greater uptake by plant roots [51-53].
In our trial, the inoculation with biofertilizer bacteria (Azotobacter or Cyanobacteria or Azotobacter + Cyanobacteria) significantly increased the concentration of macronutrients (N, P, K, Ca, Mg) and micronutrients (B, Zn, Mn, Fe, Cu) across all treatments. Due to their ability to fix nitrogen in the soil and increase plant and soil fertility, cyanobacteria and azotobacter were reported to significantly impact the growth of crop plants [54]. The plant growth in terms of root and shoot development was further enhanced by inoculating cyanobacteria with azotobacter. Similar results in increasing root and shoot growth were observed in drought-stressed plants subjected to inoculation with both plant growth-promoting rhizobacteria and cyanobacteria [55]. Cyanobacteria and Azotobacter tend to play essential roles in producing a diverse array of extracellular chemicals that promote plant growth, release several nutrients, plant growth regulators [56], amino acids and vitamins [57], polysaccharides [18], and anti-microbial products [58]. These substances were reported to influence plant development and yield, either directly or indirectly.
Table 5.
The effects of N-fixing bacteria and N fertilization on the main essential oil composition of Clary sage plants.
[i] Note: †Data followed by the same letter in a column are not significantly different according to ’Tukey’s honestly significant difference (HSD) test at P ≤ 0.05, NFB: Nitrogen fixing bacteria, T1: 120 kg N ha−1 without NFB, T2: 120 kg N ha−1 + Azotobacter, T3: 120 kg N ha−1 + Cyanobacteria, T4: 120 kg N ha−1 + Azotobacter + Cyanobacteria, T5: 60 kg N ha−1 without NFB, T6: 60 kg N ha−1 + Azotobacter, T7: 60 kg N ha−1 + Cyanobacteria, and T8: 60 kg N ha−1 + Azotobacter + Cyanobacteria.
Table 6.
Correlation matrix analysis of different response variables of clary sage grown under N-fixing bacteria and N fertilization regimes.
[i] Note: Nitrogenese Nase, dehydrogenase activity DAH, nitrogen N, phosphorous P, potassium P, calcium Ca, magnesium Mg, boron B, zinc Zn, manganese Mn, iron Fe, copper Cu, chlorophyll fluorescence Fv/Fm, chlorophyll content SPAD, normalized difference vegetation index NDVI, leaf area LA, and shoot dry weight SDW.
Moreover, plants inoculated through Bacillus subtilis, Pseudomonas fluorescens, Cyanobacteria, or Trichoderma improved the values of Fv/Fm, SPAD-value, and NDVI [1]. It might be inferred that nutritional element variations correlate with photosynthetic parameters and pigments (e.g., Fv/Fm and SPAD value). Except for B, our study revealed a strong influence of employed treatments (N fertilizer doses and bacteria) on the SPAD or Fv/Fm and all the nutrients (K, N, P, Mg, Ca, Mn, Zn, Fe, and Cu) examined. Growth-promoting bacteria played their role in solubilizing essential nutrients and enhancing the ability of plants to uptake nutrients, which led to improved physiological activities and enhanced the pigment content in the leaves of plants [1]. An earlier study recommended using NDVI as a selection criterion under favorable growth conditions to boost wheat grain production [59]. Likewise, GreenSeeker’s output (NDVI) was used to predict early vigor, dry matter, growth rate, soil coverage, and yield [60]. The LA is a good indicator of the capacity of a plant to produce dry matter. The total leaf area of a plant was observed to vary depending on factors such as improved plant nutrition, architectural characteristics, radiation usage efficiency, radiation interception capacity, and variations in leaf number and size. In this study, inoculation with Azotobacter, Cyanobacteria, or Azotobacter + Cyanobacteria led to a significant increase in leaf area. This finding is supported by a previous study that highlighted an improved leaf area in response to mycorrhizae inoculation [61].
The inoculation-associated increased plant growth could be attributed to the capacity of microalgae to rebuild the natural nutrient cycles of soil, enhance soil organic matter, enrich plants with various nutrients and hormones, and/or to the ability of Cyanobacteria and Azotobacter to fix atmospheric nitrogen [62-64]. Cyanobacteria have been reported to interact intimately with wheat roots and significantly stimulate their growth [65]. Additionally, cyanobacterial decomposition caused mineralization of organic N, which led to greater above-ground and below-ground growth of crop plants [66]. Our findings revealed that inoculation with biofertilizer bacteria (Azotobacter or Cyanobacteria or Azotobacter + Cyanobacteria) considerably increased the nitrogenase activity, DHA, essential oil composition, photosystem II (PSII), and chlorophyll content. According to [67], inoculation with microbes positively affected the leaf area and dry matter production of plants. Moreover, Azotobacter inoculation remained effective in boosting plant growth, dry weight, yield, and total N content [68]. Previously, it has been inferred that for dry matter production, nitrogen played a strategic role compared to other macronutrients [6], as in our study, lower N fertilizer application resulted in reduced leaf area, and consequently, the plant’s dry weight was significantly reduced. Inoculation of Bacillus subtilis, Pseudomonas fluorescens, Cyanobacteria, or Trichoderma in clary sage plants significantly increased the total dry weight yield as compared to untreated control plants. Our findings confirmed that inoculation with biofertilizer bacteria (Azotobacter or Cyanobacteria or Azotobacter + Cyanobacteria) considerably increased the total dry weight of clary sage plants compared to untreated control plants. Similar results have been reported whereby inoculation with microbes improved the growth and yield of crops [68].
Other reports have also observed the effect of N fertilizer on the growth, yield, and essential oil content of medicinal plants. According to [69], 100- 150 kg N ha-1 enhanced the shoot weight and essential oil content. In our study, 120 kg ha-1 N and inoculation with biofertilizer bacteria (Azotobacter, Cyanobacteria, or Azotobacter + Cyanobacteria) considerably increased the total dry weight and essential oil content compared to untreated control plants. Although the lower dose of N (60 kg ha-1) applied in conjunction with different combinations of bacteria could not perform on par with the higher N dose in terms of essential oil production, the biofertilizer’s effectiveness in boosting the biosynthesis of essential oil might be used to reduce the mineral fertilizer’s utilization for medicinal plants like clary sage. Likewise, it has been reported that the essential oil content was enhanced by using chemical N fertilizer applied in conjunction with Azotobacter in maize grown under heavy metals’ toxicity [70]. However, inoculation with biofertilizer bacteria (Azotobacter or Cyanobacteria or Azotobacter + Cyanobacteria) significantly increased essential oil and its composition in clary sage plants, highlighting the potential of biofertilizers in reducing the application of mineral fertilizers. Related results were reported whereby Bacillus subtilis, Pseudomonas fluorescens, Cyanobacteria, or Trichoderma increased the growth of maize plants when applied with reduced doses of chemical fertilizers, and it was also inferred that the higher quantities of chemical fertilizers reduced the performance of biofertilizers [70]. Regarding the correlation matrix, macronutrients (N, P, and K) were recorded to have a positive association with micronutrients (Ca, Mg, Mn, Zn, Fe, B, and Cu), which might be owing to higher uptake of micronutrients by clary sage in the presence of greater concentrations of macronutrients. Comparable results were reported in previous studies whereby an increase in macronutrient concentrations also coincided with greater micronutrients in many field crops [7, 10, 60, 71]. Likewise, a significantly positive association of shoot fresh weight with NDVI and SPAD values could be due to higher biosynthesis of chlorophyll, which triggered the synthesis and partition of assimilates towards the shoot, and ultimately, shoot weight was increased. Previously, it was reported that higher NDVI and SPAD values corresponded to significantly greater plant weight, and it was attributed to markedly higher photosynthesis rates and partitioning of assimilates, which boosted the accumulation of biomass over a period of time [60]. Furthermore, essential oil was recorded to have a strong association with the DHA, P, K, Cu, Fv/Fm, and NDVI, indicating the crucial roles of macronutrients (particularly P and K) and micronutrients (especially Cu) along with robust vegetative growth traits (like Fv/Fm and NDVI) in increasing the essential oil content of clary sage. Thus, it could be inferred that vigorous vegetative growth and increment in macronutrient uptake played a pivotal role in boosting the essential oil biosynthesis in clary sage.
Conclusions
Based on recorded findings, it might be inferred that half-dose application of the recommended N fertilizer rate could not boost the concentration of macro- and micro-nutrients (N, P, K, Ca, Mg, B, Zn, Mn, Fe, and Cu), dehydrogenase activity, oil percentage, and main essential oil composition (camphene, β-pinene, limonene, linalool, camphor, terpineol, bomeal, bornyl acetate, eugenol, and b-caryophyllene) compared to a 120 kg ha-1 N dose. Likewise, it also resulted in reduced quantum efficiency of photosynthesis II in dark-adapted conditions, SPAD-value, NDVI, leaf area per plant, and shoot dry weight in clary sage plants. Inoculation of clary sage plants with Azotobacter, Cyanobacteria, or Azotobacter + Cyanobacteria caused a substantial improvement of all the studied traits in contrast to untreated control plants, indicating the potential of microbial utilization as an alternative to synthetic nitrogen fertilizer. Furthermore, essential oil’s strong association with the DHA, P, K, Cu, Fv/ Fm, and NDVI indicated vital roles of macronutrients (particularly P and K) and micronutrients (especially Cu) along with robust vegetative growth traits (like Fv/ Fm and NDVI) in boosting the essential oil content of clary sage. Overall, these low fertility rates highlight the importance of achieving symbiosis to lessen the reliance on fertilizers and other inputs, thereby enhancing the sustainability of cultivating aromatic-medicinal plants even on low-fertility soils. Future research needs to focus on higher doses of N and more species of biological N-fixing bacteria to develop co-application of reduced doses of mineral N fertilizer and biofertilizers as an efficient approach to achieve higher growth and oil content of clary sage. Moreover, there is a need to study the relationship among photosynthesis, nutrient concentration, and essential oils productivity of clary sage under varying N doses and different combinations of growth-promoting bacteria.

