


Introduction
The majority of industries and transportation systems currently rely heavily on petroleum resources. Oil exploration and processing generate significant amounts of wastewater and oil-containing residues. Furthermore, crude oil spills frequently occur during transportation, causing severe environmental pollution. Although spill laws and conventions have been implemented, annual statistics show a decrease in the number and size of oil spills from 1970 to 2015. These incidents continue to happen, highlighting the persistent environmental challenges associated with petroleum-related activities [1]. Statistics indicate that approximately 1.3 million tons of oil have been released into the ocean. Marine oil spills have substantial repercussions for both marine ecosystems and human health [2].
Diesel is a complex hydrocarbon derived from the distillation of crude oil and typically has a carbon number ranging between C9 and C20. It comprises various components, including paraffins, olefins, naphtha, and aromatic compounds. Accidental leaks from oil storage tanks or pipelines are a major source of diesel release into the environment [3]. The toxicity of diesel oil disrupts microbial communities crucial for biogeochemical cycles, negatively affecting a wide range of organisms. The extent and duration of oil pollution depend on factors such as the amount and composition of the oil spill and the characteristics of the affected ecosystem [4].
Bioremediation is a widely recognized, environmentally friendly, and sustainable approach for treating petroleum spills and leaks [5]. Biostimulation and bioaugmentation are two common strategies used in the mitigation and remediation of oil spills. However, the rapid dilution and leaching of water-soluble nutrients from sediment can limit their effectiveness [6]. Therefore, bioaugmentation is often a preferred method for remediating oil spills [7]. Numerous studies have demonstrated the effectiveness of bioaugmentation in achieving significant degradation. For example, bioaugmentation contributed to an impressive 79% of the overall degradation in the Gulf of Taranto oil spill [8]. Several enzymes, such as dehydrogenase (DHG) [9], manganese peroxidase (MnP), and laccase (Lac) [10], have been used in diesel degradation.
Laccase is a member of the multi-copper oxidase family found in various organisms, including plants, insects, fungi, and bacteria [11]. This enzyme can degrade a broad range of substrates such as lignin-related compounds, aliphatic compounds, and aromatic compounds using molecular oxygen [12]. On the other hand, the laccase-producing white rot fungus Coriolopsis gallica with a laccase activity of 15.26 U/mL exhibits a high diesel-degrading potential [13]. Moreover, an engineered bacterial consortium that produces laccase has demonstrated a high potential for diesel removal, achieving 79.20% [14].
A microbial fuel cell (MFC) is a bio-electrochemical technology that uses microbial metabolism to convert the chemical energy in organic matter directly into electrical energy without combustion [15]. MFCs have been used to treat various wastewaters, including dairy wastewater [16], ethanol stillage [17], municipal wastewater [18], brewery wastewater [18], swine wastewater [19], and petroleum waste [20].
In this study, diesel-degrading bacteria were selected from marine sediment. The diesel-removing capacity and enzyme profile of the bacterial consortium were evaluated when cultivated in diesel-contaminated seawater. Finally, the consortium was integrated with an MFC for electricity generation.
Experimental
Sample Collection
Marine sediment samples were collected from Samaesarn Island, Chon Buri, Thailand. All samples were stored in food-grade sterile plastic bags (Sunzip, Thailand) on ice and then rapidly transported to the laboratory at the Faculty of Science and Digital Innovation, Thaksin University, Thailand. The samples were stored at 4ºC in a refrigerator (Samsung, South Korea) until used in subsequent experiments.
Synthetic Seawater
The synthetic seawater was prepared according to Shi et al. [21]. The synthetic seawater contained 5.00 g/L of (NaCl), 0.06 g/L of (Na2HPO4), 0.05 g/L of (KH2PO4), 0.02 g/L of (CaCl2), 0.04 g/L of (FeSO4 · 7H2O), and 0.14 g/L of (MgSO4). All chemicals were purchased from HiMedia Laboratories, India. The synthetic seawater was sterilized by autoclaving (Hirayama, Japan) at 121ºC for 15 min before use.
Enrichment and Screening
4 g of sample were inoculated into 40 mL of sterile synthetic seawater supplemented with 10% (v/v) diesel in a 50 mL centrifuge tube (SPL Life Sciences, South Korea) and incubated at room temperature for 48 h with shaking at 150 rpm. This process was repeated 10 times to enrich for a consortium capable of utilizing diesel as a carbon source.
For the selection process [22], 10 mL of the 48-h enriched consortium (concentration of 1.0×10⁸ cells/mL) was added to 90 mL of diesel-contaminated seawater in a 250 mL Erlenmeyer flask (Duran, Germany). The mixture was then incubated at room temperature for 48 h with shaking at 150 rpm.
Laccase Activity
The cultures were centrifuged at 12,000 rpm for 10 min using a Microspin 12 high-speed mini-centrifuge (Biosan Laboratories, United States). The supernatants were collected in 1.5 mL DNA-free microcentrifuge tubes (Invitrogen, United States) and used for enzyme analysis. Laccase activity was measured using the 2,2’-Azino-bis (3-ethylbenzothiazoline-6-sulfonic acid) (ABTS) assay [23]. A 0.1 mL aliquot of supernatant was mixed with 0.9 mL of 0.1 M ABTS solution in sodium acetate buffer (prepared with 1.78 g/L acetic acid (CH₃COOH) and 5.77 g/L sodium acetate (CH₃COONa)). All chemicals were purchased from HiMedia Laboratories, India. The solution was incubated for 1 min, and the absorbance was measured at 420 nm. Laccase activity (U/mL) was calculated using Equation (1).
Where ΔAbs is the difference in light absorbance value at 420 nm; V is the total volume of the sample (mL); Ve is the volume of the enzyme (mL); and Δt is the incubation time (min).
Diesel Removal
For diesel removal, 10 mL of n-hexane was mixed with 100 mL of the enriched consortium in a 250 mL Erlenmeyer flask. The mixture was shaken at 150 rpm for 20 min at room temperature and then transferred to a separating funnel. The supernatant was collected in 1.5 mL DNA-free microcentrifuge tubes, and the residual diesel content was monitored using UV-Vis spectrophotometry (Shimadzu, Japan) by measuring absorbance at 225 nm [24].
Where C0 is the light absorbance value of the initial concentration, and Ct is the light absorbance value of the sample after incubation. The bacterial consortium exhibiting the highest diesel degradation potential was selected for the next phase of the study.
Effect of Initial Concentration
The 10 mL of the 48-h enriched consortium (concentration of 1.0×10⁸ cells/mL) was added to 90 mL of diesel-contaminated seawater with various concentrations (2, 4, 6, 8, and 10 g/L) in a 250 mL Erlenmeyer flask. The mixture was then incubated at room temperature for 48 h with shaking at 150 rpm [24].
Degraded Metabolites
The degraded metabolites produced by the selected bacterial consortium were analyzed using gas chromatography-mass spectrometry (GC-MS) [14]. GC-MS was performed using an Agilent 7890-5975C system (California, USA) to analyze the degraded metabolite components. Separation was achieved on an HP-5MS elastic quartz capillary column (60 m × 0.25 mm × 0.25 μm). The injection volume was 1 μL, and helium (99.999% purity) was used as the carrier gas at a flow rate of 1 mL/min. For saturated hydrocarbon analysis, the oven temperature was programmed as follows: initial temperature of 50ºC (1 min), followed by 15ºC/min to 120ºC and 3ºC/min to a final temperature of 300ºC (25 min).
Microbial Community Analysis
The 10 mL of the 48-h enriched consortium was added to 90 mL of diesel-contaminated seawater in a 250 mL Erlenmeyer flask. The mixture was then incubated at room temperature for 48 h with shaking at 150 rpm. Subsequently, the enriched consortium was transferred into 1.5 mL DNA-free microcentrifuge tubes and centrifuged at 12,000 rpm for 10 min using a Microspin 12 high-speed mini-centrifuge. The supernatant was discarded, and the cell pellet was collected.
Metagenomic DNA was extracted from a selected consortium using the PureLink™ Microbiome DNA Purification Kit (Thermo Fisher Scientific, United States) following the manufacturer’s protocol. DNA quality and quantity were assessed via electrophoresis and spectrophotometry with a NanoDrop instrument. The V3 and V4 regions of the 16S rDNA gene were amplified using PCR with primers and cycling conditions [25].
MFC Operation
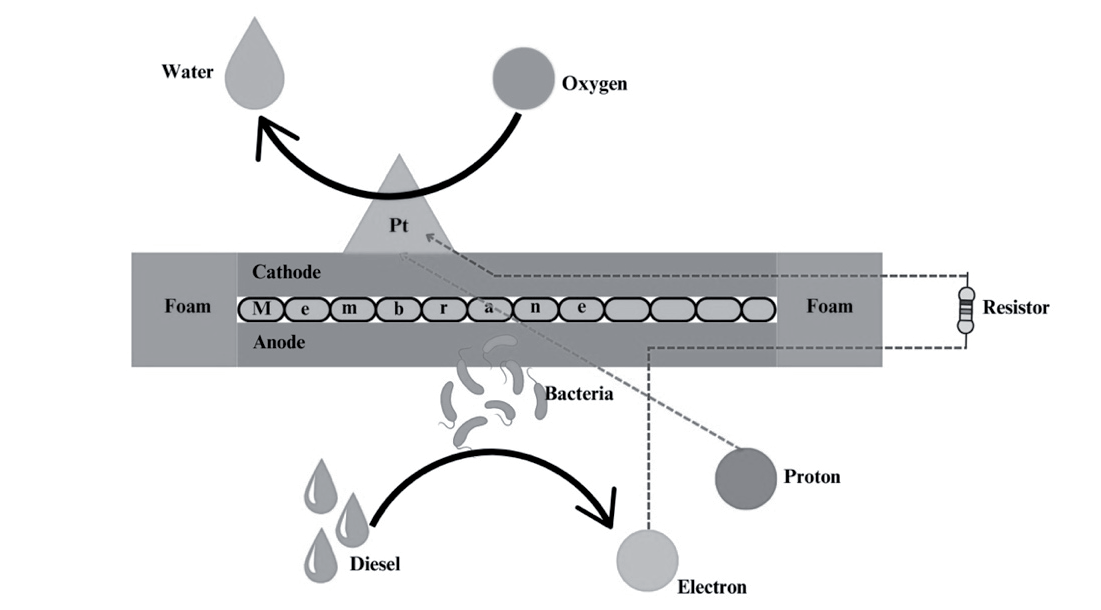
The floating MFC was set up according to the MFC model described in a previous study [22]. Fig. 1 shows a diagram of the floating MFC used in this study. The 4 cm² Microwave-treated graphite plates served as the anode [26]. The cathode consisted of 4 cm² Pt-coated carbon cloth. A 2 mm thick ceramic plate served as the ion exchange membrane [27]. Polyethylene foam provided buoyancy. The 900 mL of 2% (v/v) diesel-contaminated seawater was placed in a 1.5 L square glass chamber, and 100 mL of a 48-h enriched consortium was added. The open-circuit voltage (OCV) was recorded every 60 min for 48 h. The closed-circuit voltage (CCV) was monitored under varying resistances from 300-5,000 Ω to generate a polarization curve. Electrochemical properties were calculated using Ohm’s law. The diesel degradation was evaluated.
The electrochemical properties were calculated as follows:
Where I is the current (A), V is the close circuit voltage (V), R is the external resistance (Ω), P is the power (W), CD is the current density (A/m3), A is the working volume (m3) or electrode area (m2), and PD is the power density (W/m3).
Results and Discussion
Laccase Activity
The enrichment process revealed that only six bacterial communities could survive in synthetic seawater amended with 10% (v/v) diesel without the addition of an external carbon source. This suggests that the enriched bacterial consortium can utilize diesel as a carbon source for growth by secreting degradative enzymes to break down the diesel hydrocarbons.
The supernatant of enriched synthetic seawater was collected for the monitoring of laccase activity using a colorimetric method by ABTS assay. The results found that the bacterial consortium MS had the highest laccase activity with 28.13±0.20 U/mL, followed by SS, MN, SW, MW, and FF with 25.00±0.11, 22.21±0.08, 18.36±0.47, 15.00±0.10, and 5.32±0.19 U/mL, respectively (Fig. 2).
Laccases are a class of multi-copper oxidases that possess a remarkable ability to oxidize a diverse array of phenolic and non-phenolic compounds, making them valuable tools in various biotechnological applications [28]. Bacterial laccases are gaining prominence in industrial settings due to their superior characteristics compared to their fungal counterparts. These advantages include broader temperature and pH operating ranges, coupled with enhanced stability against inhibitory agents [29].
Several studies have highlighted the potential of bacterial laccases. Khaled et al. isolated a laccase-producing bacterium from soil capable of degrading azo dyes, achieving degradation rates between 89.21% and 91.69% under laboratory conditions [30]. Similarly, Ambika et al. isolated laccase-producing bacteria from decaying plant soil and glacial lake sediment, observing a maximum laccase activity of 0.029 U/mL [31]. Furthermore, Kumar and Chandra isolated Bacillus cereus from sludge, revealing a laccase activity of 6.09 U/mL and its potential application in the biodegradation of pulp and paper mill wastewater [32].
Diesel Degradation
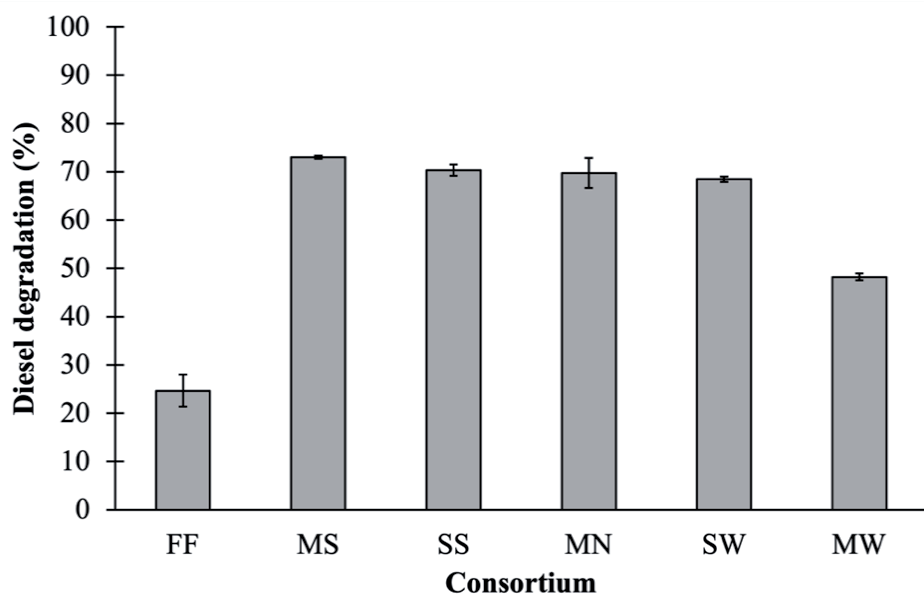
Diesel degradation was studied using UV-Vis spectroscopy, and the degradation rate was calculated. The bacterial consortium MS achieved the highest diesel degradation, reaching 73.00%±0.33%. This maximum degradation occurred when the consortium was inoculated into 10% (v/v) diesel-contaminated synthetic seawater and incubated at room temperature for 48 h without the addition of exogenous media (Fig. 3).
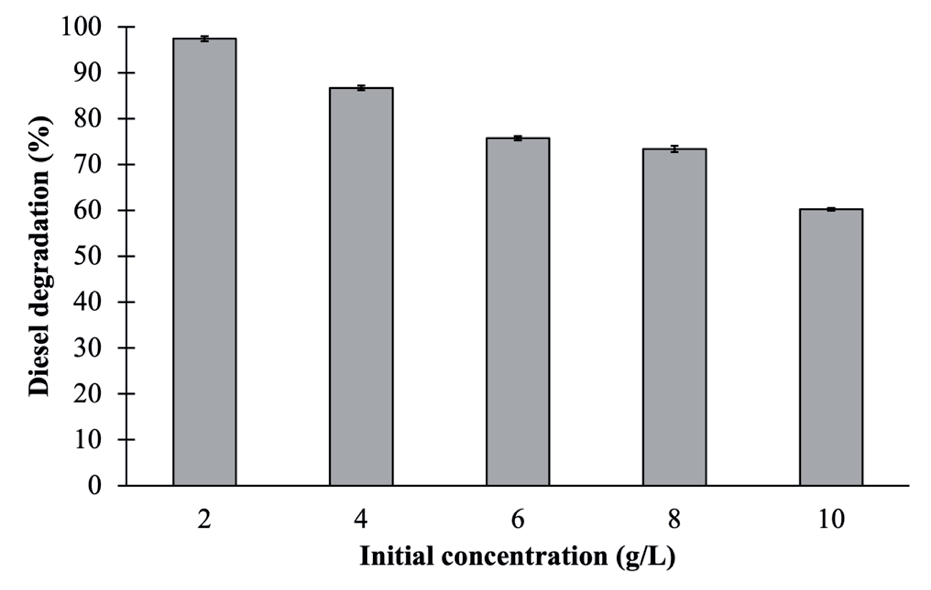
The effect of initial diesel concentration ranging from 2 to 10 g/L was investigated. The highest diesel degradation of 97.38%±0.53% was observed when the initial diesel concentration was 2 g/L. This result was achieved after a 48 h incubation period without the addition of any chemicals or media (Fig. 4).
Fig. 2.
Laccase activity of enriched bacterial consortia in diesel-contaminated seawater. The consortium enriched from floating foam (FF), marine net (MN), sea sand (SS), sediment (SW), and plastic waste (MW).
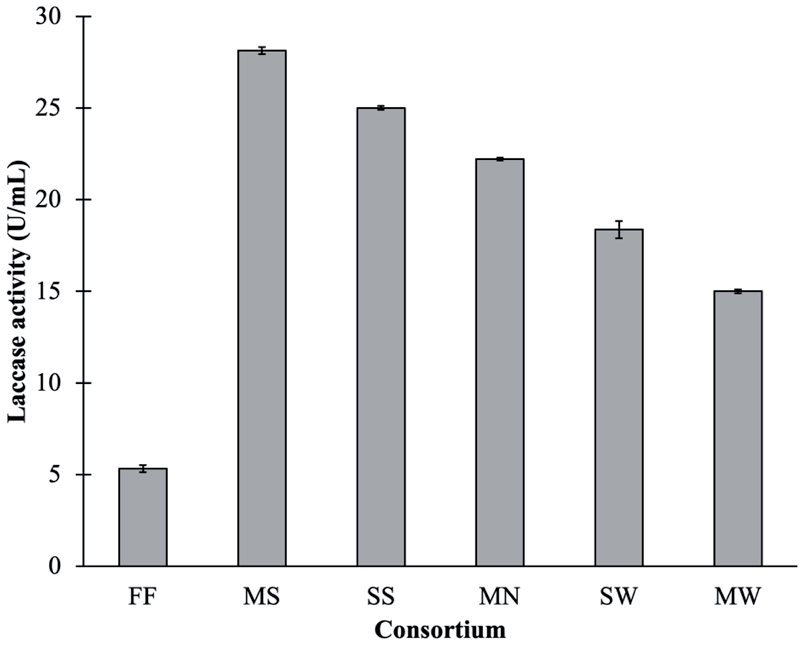
Fig. 3.
Diesel degradation (%) of enriched bacterial consortium in diesel-contaminated seawater. The consortium enriched from floating foam (FF), marine net (MN), sea sand (SS), sediment (SW), and plastic waste (MW).
Bioremediation is a promising biological technology for treating hydrocarbon-contaminated environments due to its prominence, environmental friendliness, cost-effectiveness, efficiency, and ease of application [33]. Several studies have demonstrated the effectiveness of this approach. Bao et al. isolated marine bacteria from petroleum-contaminated seawater and mud, achieving a maximum crude oil degradation of 79.00% in a 14-day laboratory-scale experiment at 25°C with shaking and an initial crude oil concentration of 0.1% (v/v) [2]. Dai et al. utilized a laccase-producing bacterium for heavy oil and diesel degradation in a stimulation pool, reporting a maximum degradation rate of 66.50% after 100 days of remediation [14]. Similarly, Bekele et al. isolated diesel-degrading bacteria from hydrocarbon-contaminated soil, achieving 84.00% diesel degradation in a 15-day culture with 0.5% (v/v) initial diesel concentration [34]. Furthermore, Zhou et al. immobilized a biosurfactant-producing bacterium isolated from cold-seep sediment onto biochar for diesel degradation in contaminated seawater. This approach yielded a maximum diesel removal of 94.70% after a 7-day incubation period [35].
Degraded Metabolites
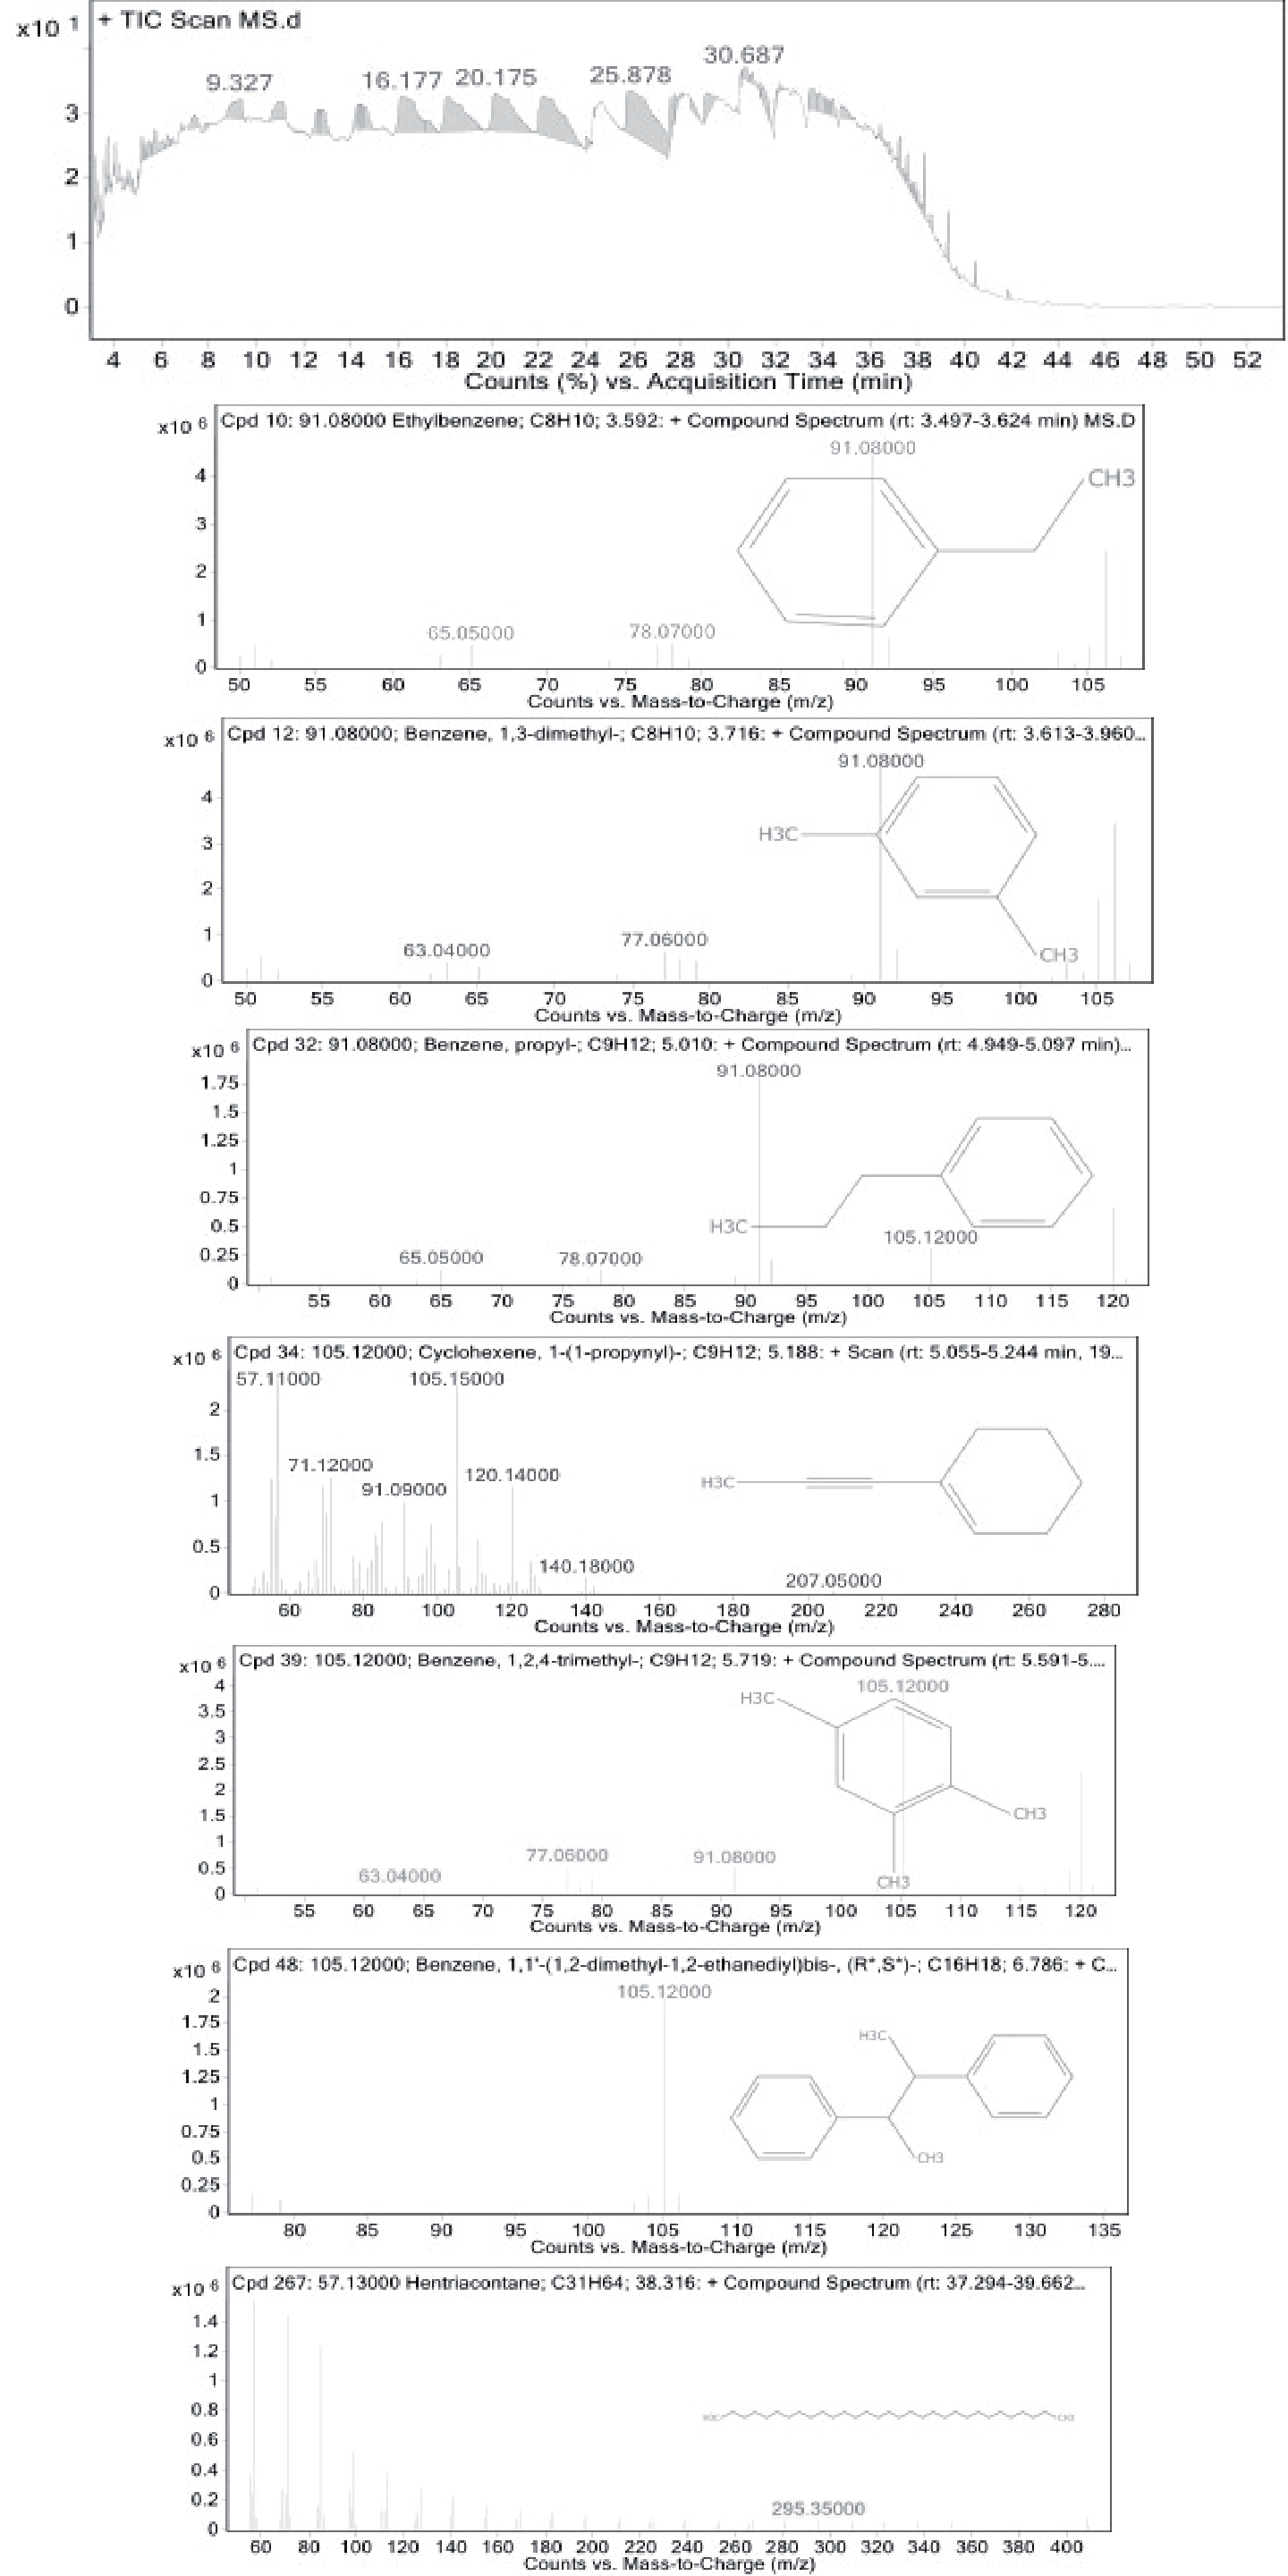
Following the degradation process, diesel-degraded metabolites were monitored using GC-MS. The chromatogram of these metabolites is shown in Fig. 5. Identified metabolites included ethylbenzene, 1,3-dimethylbenzene, propylbenzene, 1-(1-propynyl)-1- cyclohexene, 1,2,4-trimethylbenzene, benzene,1,1’-(1,2- dimethyl-1,2-ethanediyl) bis, and hentriacontane.
Previous research has demonstrated that certain metabolites produced by the MS bacterial consortium, such as ethylbenzene, exhibit high vapor pressure and low solubility. Consequently, if released into aquatic environments, these compounds are susceptible to photodegradation by sunlight with an estimated half-life in air of 2 days [36].
The presence of 1,3-dimethylbenzene is noteworthy. Mohamadpoor et al. reported the production of this compound by the bacterium Achromonas xylosoxidans, isolated from bean roots, and suggested its potential use in biocontrol of the fungal plant pathogen Fusarium solani [37]. Another identified metabolite, propylbenzene, has been detected as a volatile organic compound associated with petrochemical pollution in groundwater [38]. Furthermore, Li et al. demonstrated the successful biodegradation of 1,2,4-trimethylbenzene in contaminated seawater using the marine microalga Chaetoceros sp. [39]. The benzene,1,1’-(1,2-dimethyl- 1,2-ethanediyl) bis has been shown to possess potential in vitro antioxidant properties [40]. Finally, hentriacontane, which is a long-chain alkane, has been detected. It has been reported to exhibit antimicrobial activity [41]. The presence and potential implications of these various metabolites warrant further investigation.
Bacterial Community
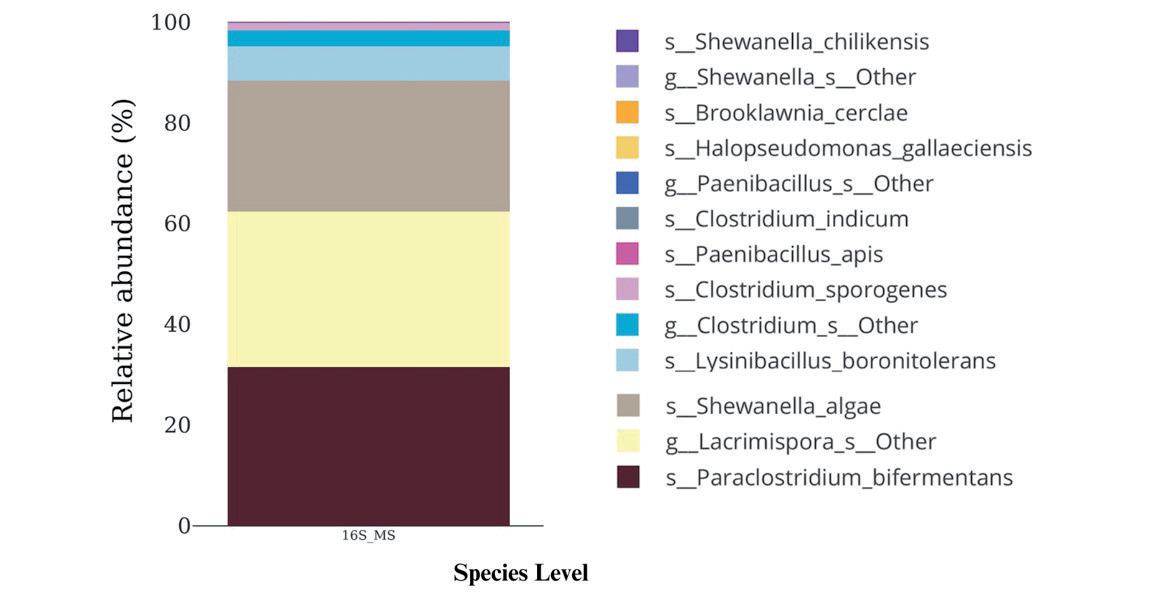
The MS bacterial consortium with the highest diesel degradation community was subjected to 16S rDNA gene amplification. The V3-V4 region was sequenced using an Illumina MiSeq platform. Bioinformatic tools designed for NGS data analysis were used to process all resulting sequences. The diversity results were shown in Fig. 6.
The phylum distribution of 73.982% is similar to the phylum Bacillota, followed by 26.015% of the phylum Pseudomonadota and 0.03% of Actinomycetota, respectively.
The class distribution of 67.149% is similar to Clostridia, followed by Gammaproteobacteria (26.015%), Bacilli (6.833%), and Actinomycetes (0.003%).
The order distribution of 31.535% is similar to Peptostreptococcales, followed by Lachnospirales (30.867%), Alteromonadales (25.997%), Bacillales (6.833%), Pseudomonadales (0.017%), and Propionibacteriales (0.003%).
The family distribution of 31.535% is similar to Peptostreptococcaceae, followed by Lachnospiraceae (30.867%), Shewanellaceae (25.997%), Bacillaceae (6.786%), Clostridiaceae (4.747%), Paenibacillaceae (0.047%), Pseudomonadaceae (0.017%), and Propionibacteriaceae (0.003%).
The genus distribution of 31.535% is similar to Paraclostridium, followed by Lacrimispora (30.867%), Shewanella (25.997%), Lysinibacillus (6.786%), Clostridium (4.747%), Paenibacillus (0.047%), Halopseudomonas (0.017%), and Brooklawnia (0.003%).
The species distribution showed the consortium MS mainly contains Paraclostridium bifermentans (31.535%), followed by Lacrimispora sp. (30.867%), Shewanella algae (25.990%), Lysinibacillus boronitolerans (6.786%), Clostridium sp. (3.197%), Clostridium sporogenes (1.520%), Clostridium indicum (0.029%), Paenibacillus apis (0.029%), Paenibacillus sp. (0.017%), Halopseudomonas gallaeciensis (0.017%), Brooklawnia cerclage (0.003%), Shewanella chilikensis (0.003%), and Shewanella sp. (0.003%).
Several studies have highlighted the potential of various bacterial species for bioremediation of crude oil and petroleum hydrocarbons. Shlimon et al. identified Paraclostridium sp. as a key component of a bacterial consortium capable of achieving 90% crude oil degradation in samples from the Kurdistan region of Iraq, although this process required a lengthy incubation period of 100-200 days. This suggests that while effective, the natural degradation process may be slow [42].
Other research has focused on the hydrocarbon-degrading capabilities of marine bacteria. Guo et al. demonstrated the high potential of Shewanella algae for hydrocarbon degradation under laboratory conditions [43]. Furthermore, Gharaei et al. indicated that Shewanella algae produces biosurfactants, which likely contribute to its oil degradation capacity by increasing the bioavailability of hydrocarbons. Biosurfactant production appears to be a common mechanism employed by hydrocarbon-degrading bacteria [44]. For instance, Walter et al. reported that Lysinibacillus boronitolerans, isolated from an automobile mechanic workshop soil, also produces biosurfactants facilitating oil degradation [45]. Hernandez-Santana and Dussan showed that Lysinibacillus boronitolerans achieved an 84.10% removal rate of petroleum hydrocarbons in mineral salt medium after 50 days [46].
Beyond individual species, research has also explored the role of bacterial communities and specific genera. Hirano et al. found that Clostridium sp. isolated from marine sediment promotes crude oil aggregation, which can be a valuable asset in bioremediation strategies by concentrating the oil for easier removal or further degradation [47]. Similarly, Paenibacillus sp. has shown promise in diesel degradation from soil samples [48]. This genus has also been implicated in biosurfactant production and the degradation of polycyclic aromatic hydrocarbons (PAHs), suggesting a broad range of potential applications in bioremediation [49].
Electrochemical Properties
A floating MFC was employed to recover electrons generated during diesel degradation. The floating MFC anode compartment was inoculated with a diesel-degrading consortium MS, acclimated in synthetic seawater contaminated with 2% (v/v) diesel.
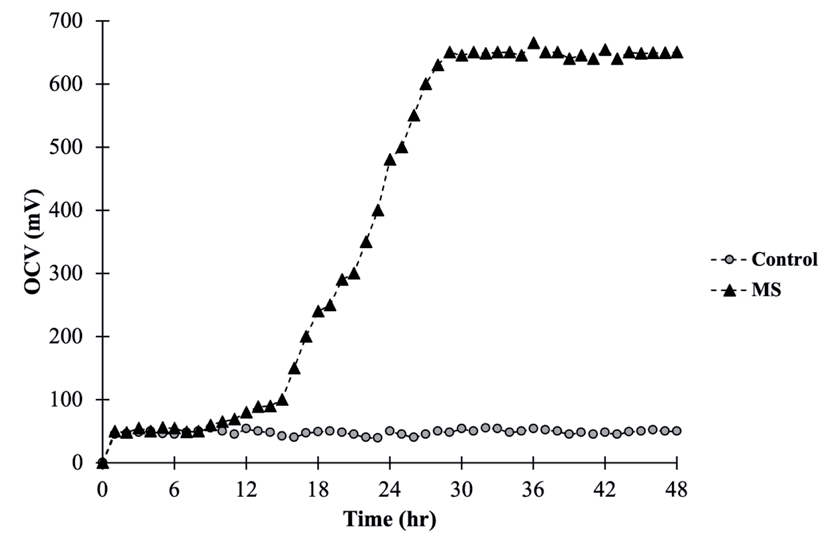
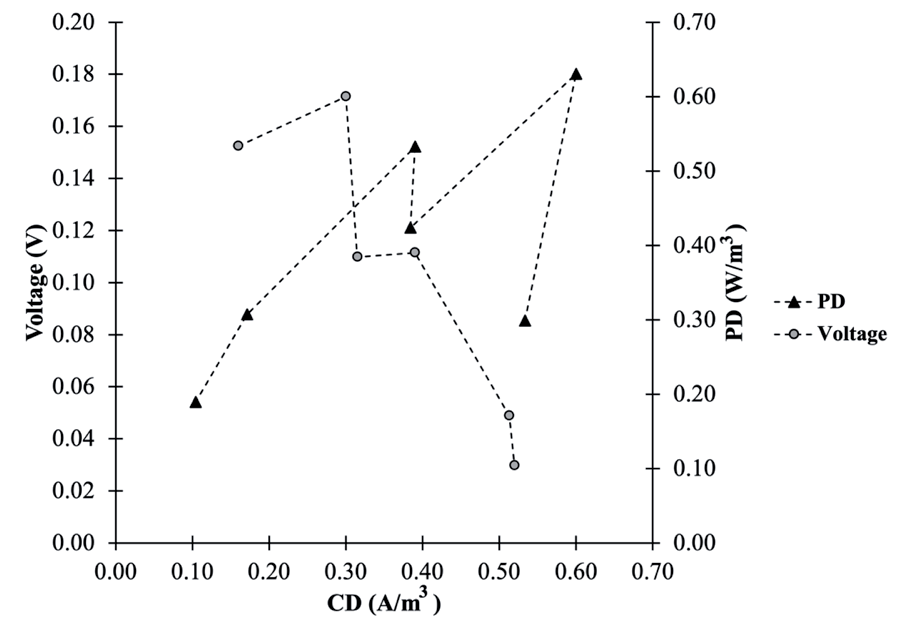
The OCV ranged from 0-90 mV during the lag phase, increased to 90-650 mV during the log phase, and stabilized at 640-650 mV during the stationary phase (Fig. 7). Closed-circuit voltage was monitored across various resistors ranging from 300 Ω to 5,000 Ω. The polarization curve of the floating MFC with MS is shown in Fig. 8. The maximum PD and CD normalized to electrode area were 0.45±0.01 W/m² and 1.50±0.00 A/m², respectively. When normalized to working volume, the maximum PD and CD were 0.18±0.00 W/m³ and 0.53±0.01 A/m³, respectively. The system achieved a diesel removal efficiency of 97.85±0.52%.
Several studies have explored the use of MFC coupled with bioremediation for simultaneous electricity generation and diesel degradation. Michu et al. employed a floating MFC inoculated with a bacterial consortium MB11 comprising Enterococcus faecalis, Proteus mirabilis, Pseudomonas aeruginosa, Raoutella planticola, Enterobacter soli, and Oceanotoga teriensis. This system achieved a maximum power density of 0.16±0.02 W/m³ alongside a diesel degradation of 53.77±0.59% [22].
Zafar et al. investigated the use of an air-cathode MFC for diesel remediation and electricity generation by a bacterial strain such as Bacillus sp., Paenibacillus sp., and Ochrobactrum sp. Their system achieved a significantly higher maximum current density of 431.10 A/m³. However, this design’s structural costs limit its applicability in marine environments [50]. While the aforementioned studies focused on consortia, Basu et al. investigated the electrogenic potential of a single species, Paraclostridium sp. AKS46. This species demonstrated a high potential for electricity generation, reaching 0.632 A/m² [51].
Conclusions
This study successfully demonstrated the bioremediation potential of a marine bacterial consortium MS for diesel contamination coupled with the recovery of electrical energy through an MFC. The consortium exhibited significant laccase activity (28.13±0.20 U/mL), which likely played a key role in its efficient diesel degradation. Notably, MS achieved a high diesel removal efficiency of 97.38%±0.53% within 2 days at an initial diesel concentration of 2 g/L without any external supplements. Integrating this consortium with a floating MFC allowed for the simultaneous recovery of electrical energy during the bioremediation process. The system achieved a maximum PD of 0.18±0.00 W/m³ and a maximum CD of 0.53±0.01 A/m³, while maintaining a high diesel removal efficiency of 97.85±0.52%. These findings highlight the potential of combining bioremediation with MFC technology for sustainable and efficient treatment of diesel-contaminated environments, offering both pollutant removal and energy generation.

