


Introduction
Owing to climate change, crop plants in their agro-environment are subjected to diverse stressors such as salinity, unsuitable temperature, and drought, which have adverse impacts on plant production [1]. Climate change is a serious problem for agriculture, because of its direct negative impact on food security. Thus, the phenomenon of climate change occupies a global concern for international organizations, especially those associated with extreme weather phenomena such as drought, and the solutions available to their management for the most affected countries [2, 3]. Regarding drought, it is well documented that sugar beet yield and quality drooping are associated with water deficiency. Irrigating crops with water less than their requirements, which is called deficit irrigation, is a crucial tactic to face low water resources and supplies. For saving and rationing agricultural water, the pattern of deficit irrigation is practiced when growing various crops [4]. However, sugar beet is negatively influenced by water deficiency, specifically at the early growth stage of the life cycle. Numerous studies illustrated the reduction in growth and yield owing to exposure to the scarcity of water [5] when harmful molecules accumulate (called reactive oxygen species, ROS), injuring the plant cells [6].
Stomata are closed, and leaf pigments are lost, resulting in a reduced rate of photosynthesis under various degrees of drought stress [7]. Application of full irrigation achieved the maximum stomatal conductivity and photosynthesis rates [8], while lowering irrigation water below normal led to a sugar yield decline as well as increases in potassium, alfa amino N, and sugar percent [9]. Then, huge efforts should be devoted to managing water deficit-based irrigation programs, keeping in mind economical and environmentally friendly approaches.
Chitosan is regarded as a secure and costless material obtained from chitin, the major component of arthropod exoskeletons and the second-most renewable carbon source [10]. Several reports pointed out that chitosan provokes various defense responses and stimulates plant drought tolerance. Chitosan improved drought tolerance by collecting stress-protective osmolytes. Chitosan motivates the antioxidant enzymes and hydrogen peroxide signaling pathways, hence participating in the sweeping of ROS [11]. The exogenous addition of chitosan remarkably increases phenolic and flavonoid compounds that perhaps destroy the coalition of free radicals and hydrogen peroxide while activating the antioxidants in this way [12]. Furthermore, chitosan enhances plant growth by enhancing water and mineral uptake and the accumulation of photosynthetic pigments [13]. Accordingly, plant height, leaf weight, dry biomass accumulation, and yield were boosted via leafy supplementation of chitosan under abiotic stress [14]. Applying chitosan as an eco-friendly component before planting by soaking seeds and through the vegetative stage by foliar application as a combination treatment at 500mg/L., resulted in the highest grain yield and its component; furthermore, the chitosan levels raised the protein and phenol content [15].
Despite the favorable effect of chitosan on several crop plants, there is scarce information available regarding its protective role in stimulating the defensive mechanism of sugar beet under diversified drought stress levels. Herein, we hypothesized that chitosan could have the potential to shrink the adverse effects of water deficiency. Then, this work aimed to assess the significance of chitosan in improving sugar beet yield and sugar profile, either in fully irrigated or droughty conditions.
Materials and Methods
Location Description
A field study was performed during the winter seasons of 2018-19 and 2019-20 at a private agricultural area situated in Giza governorate, Egypt. This study aimed to find out the importance of carboxymethylchitosan for manipulating the enzyme activity, stomatal conductivity, and marketable product of sugar beet either with well water or deficit water conditions. Soil analysis was done according to Black et al. and Jackson [16, 17]. The analysis showed that the soil was sandy, having sand (92.1%), silt (4.7%), clay (3.2%), bulk density (1.69 g cm-3), pH (8.0), ECe (1.16 dS m-1), organic matter (0.2%), available N (30.5 mg kg-1 soil), available P (4.3mg kg-1 soil), and available K (87.0mg kg-1 soil). Soil saturation percentage, field capacity, wilting point, and available water were 22.5, 12.3, 5.1, and 7.2%, respectively.
Trial Procedures
The treatments were distributed in a split-plot arrangement three times. Irrigation patterns were implemented in the main units, including 100%, 80%, and 60% of actual crop evapotranspiration at (W100, W80, and W60, respectively). The subplots were occupied by chitosan treatments (without tap water and with 200 mg L−1). Two equal doses of chitosan were sprayed at 6 and 8 weeks after sowing (WAS). Water was used as a solvent and a carrier for a spray solution of 720L ha−1
The carboxymethyl chitosan was purchased by import through the Egyptian Chemical Company (the product is made in China). The chitosan source was the shrimp exoskeletons, and its characteristics were a degree of deacetylation of 90%, a molecular weight of 4.5 kDa, and a pH of 6, with the highest solubility.
Irrigation Schedule
Using the average of the previous 7 years of climate data taken from CLAC, ARC, and Egypt, the reference (ETo) and crop evapotranspiration (ETc) were calculated using the FAO Penman–Monteith equation [18]. Plants received water amounts through the trickle irrigation system, which had a dripper inflow of 4.0 L hr−1, a pressure of one bar, and a 30.0 cm dripper spacing.
Crop Cultivation
During the initial land layout, approximately 400 kg ha−1 of ordinary superphosphate was incorporated. The experimental area involved 18 experimental units; each of them has a size of 24 m2 and includes 4 ridges with 0.6 m width and 10.0 m length. At the beginning of October in each season, sugar beet seeds were drilled. The distance between hills was 25 cm and at 4 WAS, the seedlings were thinned into one plant/hill. A multi–germ sugar beet cultivar called ‘Hamza’ obtained from the Sugar Crops Research Institute, Agricultural Research Center, Egypt, was used. Five equal portions of nitrogen fertilizer, with a total amount of 288 kg N ha−1 were added at 4, 6, 8, 10, and 12 WAS using ammonium nitrate. With the last three portions of nitrogen, a quantity of potassium sulfate (115 kg K2O ha−1) was equally applied.
Enzymatic Activity
The leaves of ten plants were obtained randomly per trial unit at 110 DAS to estimate the enzymes catalase (CAT), glutathione peroxidase (GPX), and total flavonoids (ug Rutin equivalent/100 g fresh weight) according to spectrophotometric methodology [19-21].
Leaf Stomata, Pigments, and Agronomic Traits
A sample of fully expanded leaves was collected at 110 DAS to assess the stomata traits (closure and pore area µm) by using the Scanning Electron Microscope. Further, a Li–Cor area meter LI-3000 was used to measure leaf area. Plant pigments were estimated, according to Wettestien [22]. At maturity (210 DAS), 10 plants per treatment were unbiasedly uprooted to evaluate the fresh weights of shoots and roots. Furthermore, root yield ha−1 was estimated by collecting all plants per plot.
Quality of Sugary Juice and Sugar Yield
In fresh sugar beet root samples, sucrose % and impurity contents were estimated. A Saccharometer was used to measure sucrose % [23]. Alfa amino nitrogen, sodium, and potassium, as well as extracted sugar % and sugar lost to molasses % were assessed [24-26]. Moreover, sugar yield was computed via root yield x extracted sugar %.
Water Use Efficiency (WUE)
Water use efficiency (WUE) values as kg sugar/m3 water applied were calculated for each treatment after harvesting using the following equation [27]: WUE = sugar yield (kg)/applied irrigation water (m3)
Statistical Analysis
Depending on the methods clarified by Casella via the applications of MSTAT–C program software, the combined seasonal data was analyzed [28]. To compare the averages of the tested treatments, Duncan’s multiple range test was applied at the 5% level of significance.
Results and Discussion
Catalase (CAT), Glutathione Peroxidase (GPX) Activity, and Total Flavonoids
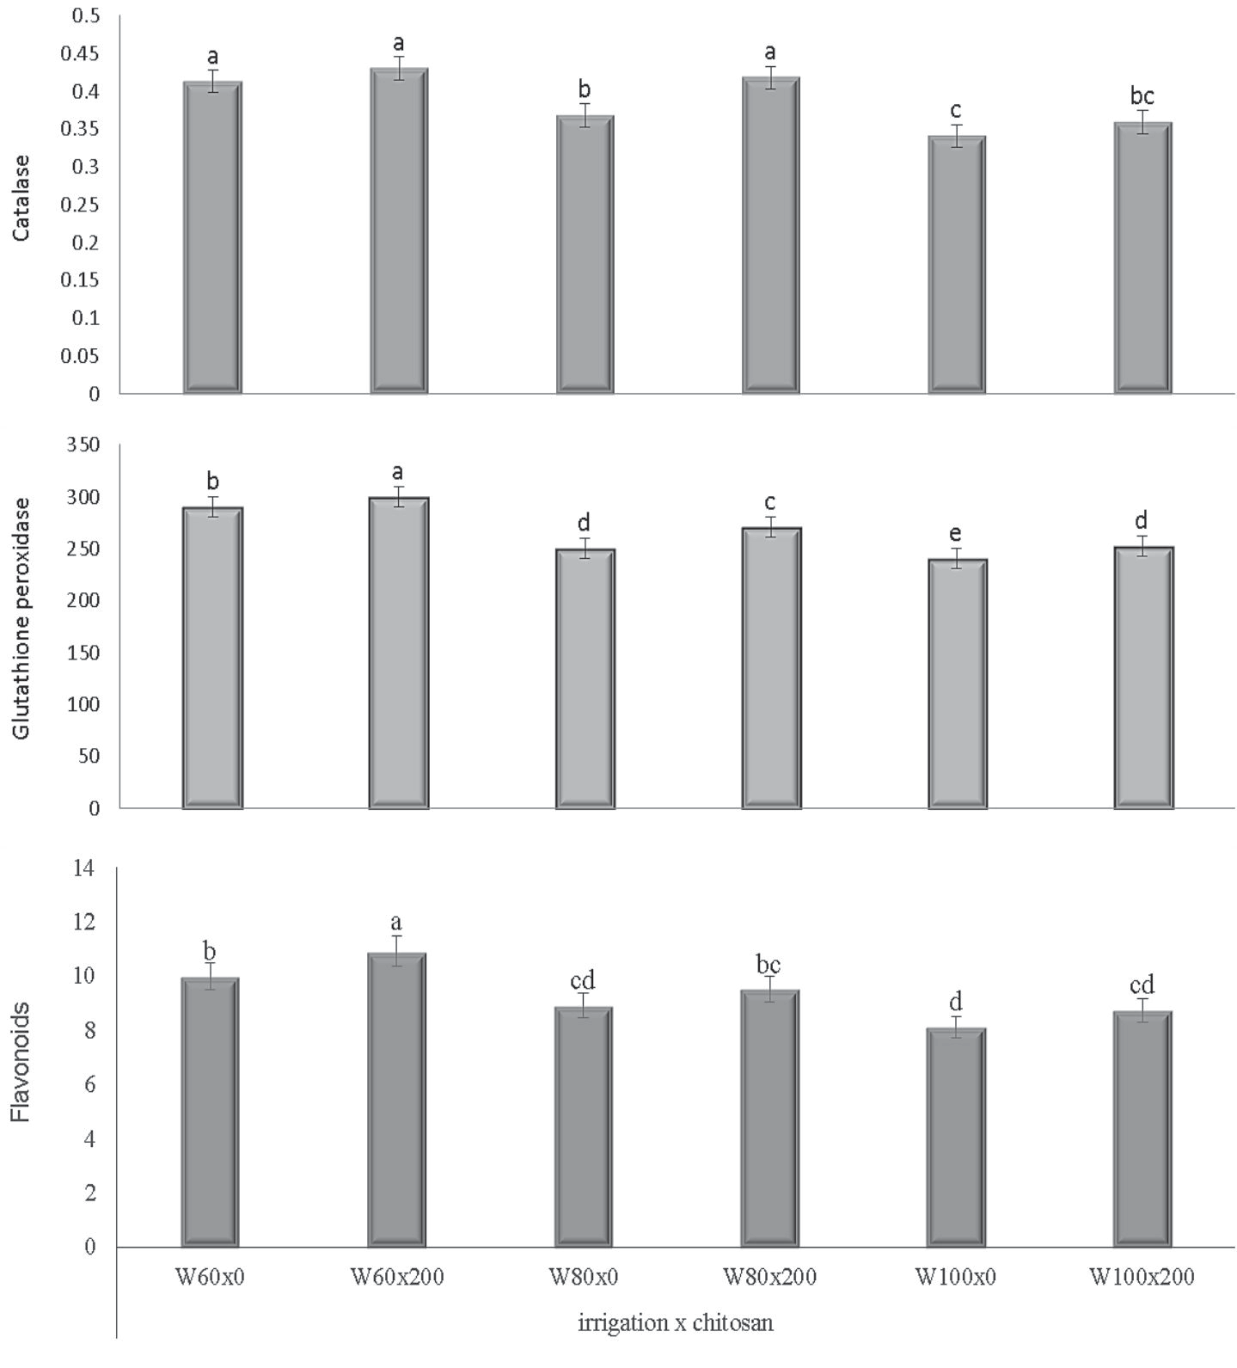
Raising water deficiency levels caused an increase in antioxidant enzyme activity, i.e., CAT, GPX, and flavonoid content, since W60 under chitosan application (200 mg L−1) showed the maximum values (Fig. 1). However, the differences between W60 x chitosan, W60 x without chitosan, and W80 x chitosan exhibited statistically similar values of CAT activity. Moreover, the values of GPX significantly increased with the application of chitosan (200 mg L−1) compared to without chitosan by 3.2, 8.08, and 4.78% under W60, W80, and W100, respectively. Plainly, supplying sugar beet plants with irrigation water <100% of crop evapotranspiration (whether W80 or W60) caused a critical disturbance in sugar beet physiological performance, stomata opening, as well as agronomic and qualitative attributes. The findings of the current work exhibited remarkable increases in antioxidant enzymes (CAT and GPX) and flavonoids when beet plants were exposed to water-deficit conditions. The acute impact in this respect was more pronounced with irrigation of W60, where the maximum increase in CAT, GPX, and flavonoids was associated with the lowest values of stomata opening and yield characteristics. Under various stresses, over-formation of ROS is produced in plants; hence, enzymatic antioxidation is also induced as a plant defensive mechanism [29]. As a result of drought-based oxidative stress effects, particularly protein inhibition, glutathione peroxidase enzymes are considered significant markers in this respect [30]. Oxidative damage raised by drought was faced through CAT and GPX accumulation and in beet leaves [31]. Flavonoids are non-enzymatic defense systems consisting of low molecular weight that have the ability to regulate the abundance of ROS through scavenging ROS and help in the recycling of H2O2 and antioxidants to preserve the redox state homeostasis inside plants [32]. The current research proves the importance of chitosan as an alleviator of drought. The superiority of plants that received chitosan in accumulating catalase, glutathione peroxidase, and flavonoids greater than that of untreated ones (Fig. 1) revealed that chitosan is an effective compound for inducing the activity of antioxidants in sugar beets, being a hydroxylated amino group that can effectively scavenge the ROS [33]. Precious research confirmed that the production of antioxidant enzymes and metabolites increased through the application of chitosan [34]. Owing to the potential of chitosan to increase glutathione peroxidase and catalase activity as anti-stress enzymes and also flavonoids and carotenoids content as non-enzymatic defense systems, many studies observed that chitosan supply promoted plant growth and availability/uptake of water and nutrients, as well as the amount of phenolic and flavonoid content. Thereby, augmenting ROS scavenging acts [35]. Further, to motivate chlorophyll pigment synthesis and plant growth [36], physiological status was adjusted under water deficit. Foliage addition of chitosan stabilizes the cell membrane of leaves and increases the activity of enzymatic antioxidants [37].
Stomata Traits
Scanning electron microscope (SEM) images illustrated that regardless of chitosan supply (without chitosan), severe (W60), and moderate (W80) drought increased stomata closure by 145.7 and 59.3% (Fig. 2) and decreased pore area by 92.0 and 11.5% (Fig. 3) compared to well-watered conditions, respectively. Using chitosan increased the opening of stomata by 12.4 and 20.3% under severe and moderate droughts, respectively. Moreover, chitosan increased pore area by approximately 8.3% with W60 and 12.3% with W80. Regulation of stomata movement is another manifestation of plant reaction to water deficiency situations. The anatomical SEM images of leaves exhibited progressive decreases in stomata opening (Fig. 2) and stomatal pore area with an increased drought level (Fig. 3). It is well known that guard cell pressure is lost under drought because abscisic acid (ABA) accumulates in leaves, causing perturbations in ionic homeostasis that oblige the ions of potassium (K+) to seep into guard cells. Accordingly, the relative water content of the leaves reduces and the stomata close (Fig 2). Furthermore, leaf area reduction under low water supply could be attributed to a weakening in the activity of cell division and elongation. Deficient growth of the shoot was associated with deficit water; hence the shoot root of the beet was dramatically decreased [38]. Concurrent with leaf area and plant pigment results (Table 1), shrinking the plant foliage relative to the root is one of the most important actions to face the adverse effects of drought [39]. Chitosan application statistically activated chlorophyll and carotenoid formation [40]. Otherwise, chitosan showed promising results related to adjusting the stomata closure and pore area in beets under water deficiency. It confirmed that under various irrigation water levels, favorable responses were achieved by providing chitosan, which increased the opening and pore area of the stomata. Several osmolytes involving organic acids and sugars, which are required for osmotic adjustment, were induced by chitosan treatment in a stressed environment [16]. Since proteins involved in carbon dioxide fixation or metabolism of energy are distinctly influenced by drought [41], chitosan positively modified this effect by relatively increasing the stomata aperture and pore area of sugar beet leaves. Thus, it is expected that the flux of CO2 through leaf stomata will increase, and consequently, the rate of photosynthesis will increase. In addition, chitosan enhanced stomatal conductance, while the reduced transpiration rate dwindled [35].
Fig. 1.
Catalase (U g−1 protein) and glutathione peroxidase (U g−1) enzymes activity, and total flavonoids (ug Rutin eq 100 g−1 fw) of sugar beet as influenced by irrigation level and chitosan (mg L−1) application. W60, W80 and W100: irrigation by 60, 80 and 100% of crop evapotranspiration, respectively. Values are the mean of 3 replicates±standard errors. Varied letters within bars signalize that there are significant differences by Duncan’s.
Plant Pigments and Agronomical Attributes
As shown in Table 1, all studied attributes of sugar beet significantly changed due to the combinations of irrigation and chitosan. In this respect, W100 was the most sturdy irrigation pattern for stimulating all agronomic attributes under chitosan supply. Under severe drought (W60), plots treated with chitosan showed increases in chlorophyll “b” and root yield of sugar beet, which amounted to 10.65 and 4.74%, respectively, higher than the untreated plots. Moreover, plots irrigated by W100 produced increases of 7.56, 9.57, 6.89, and 4.56% in chlorophyll “b”, carotenoids, top fresh weight, and root yield, respectively, with the application of chitosan compared to no chitosan spraying. Under mild drought (W80), the favorable effect of chitosan was obtained only for carotenoids, with an increase of 25.28% greater than the control (without chitosan). The changes in plant physiology and stomata anatomy certainly reflect on the economic product expressed in root yield and root traits that have been exploited as a substantiation of morphology in plants as a result of water shortage [42]. Therefore, the decrease in yield due to deficient water can be attributed to morphological responses, which make plants relatively tolerate the dry conditions, whereby the roots resort to extending downward into the soil to obtain more water. A distinct reduction in beet root yield because of moisture deficiency was documented [43]. On the contrary, the opposite effect of chitosan against stress was evident in enhancing growth and yield, whether with moderate or severe drought (Table 1). It has been noted that there was improvements in the growth of the root while improving the uptake of water and nutrients due to chitosan application, thus boosting the sugar beet yield parameters under different water regimes [37]. Furthermore, plants provided with chitosan showed better growth and development due to improved water and mineral uptake [19, 35]. The useful effect of chitosan on stimulating the growth of roots signifies its effectiveness in promoting root system absorption of more water to maintain moisture stability in the rhizosphere, which is a crucial event under drought stress. Because of the regulation of cell osmotic potential by chitosan supply, soil solution uptake increased, and consequently, the agronomical attributes were boosted [44].
Fig. 2.
The change in sugar beet stomata closure % due to application of chitosan under different irrigation regimes. W60, W80 and W100: irrigation by 60, 80 and 100% of crop evapotranspiration, respectively.
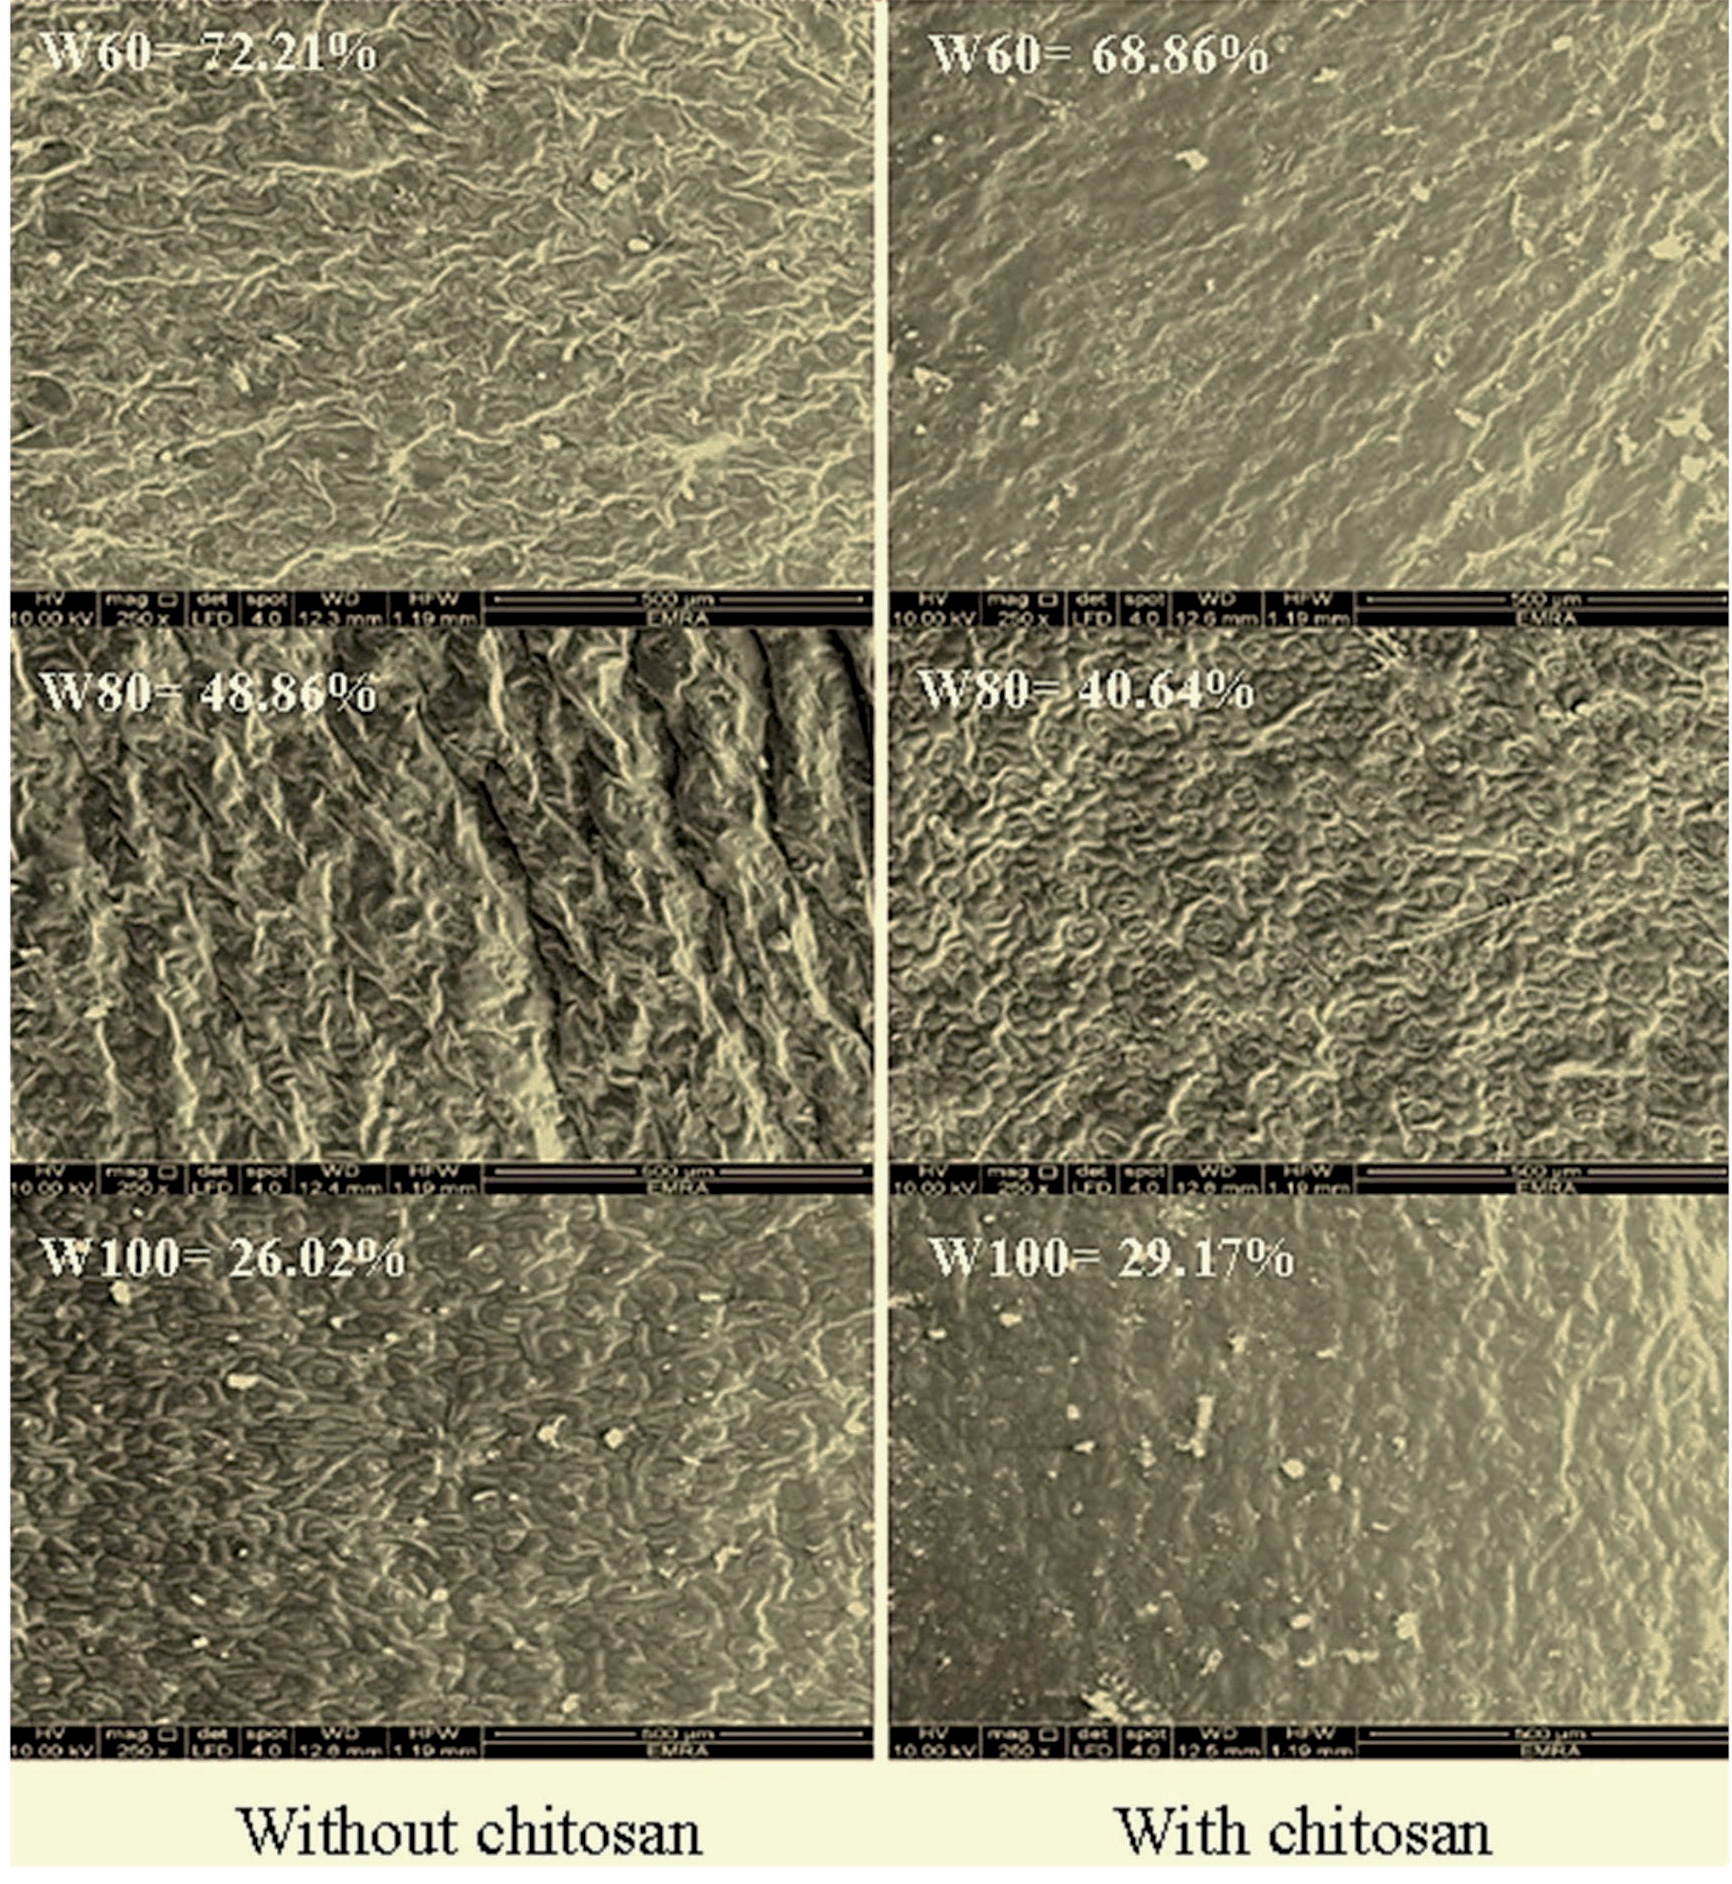
Fig. 3.
The change in sugar beet stomata pore area (μm) due to application of chitosan under different irrigation regimes. W60, W80 and W100: irrigation by 60, 80 and 100% of crop evapotranspiration, respectively.
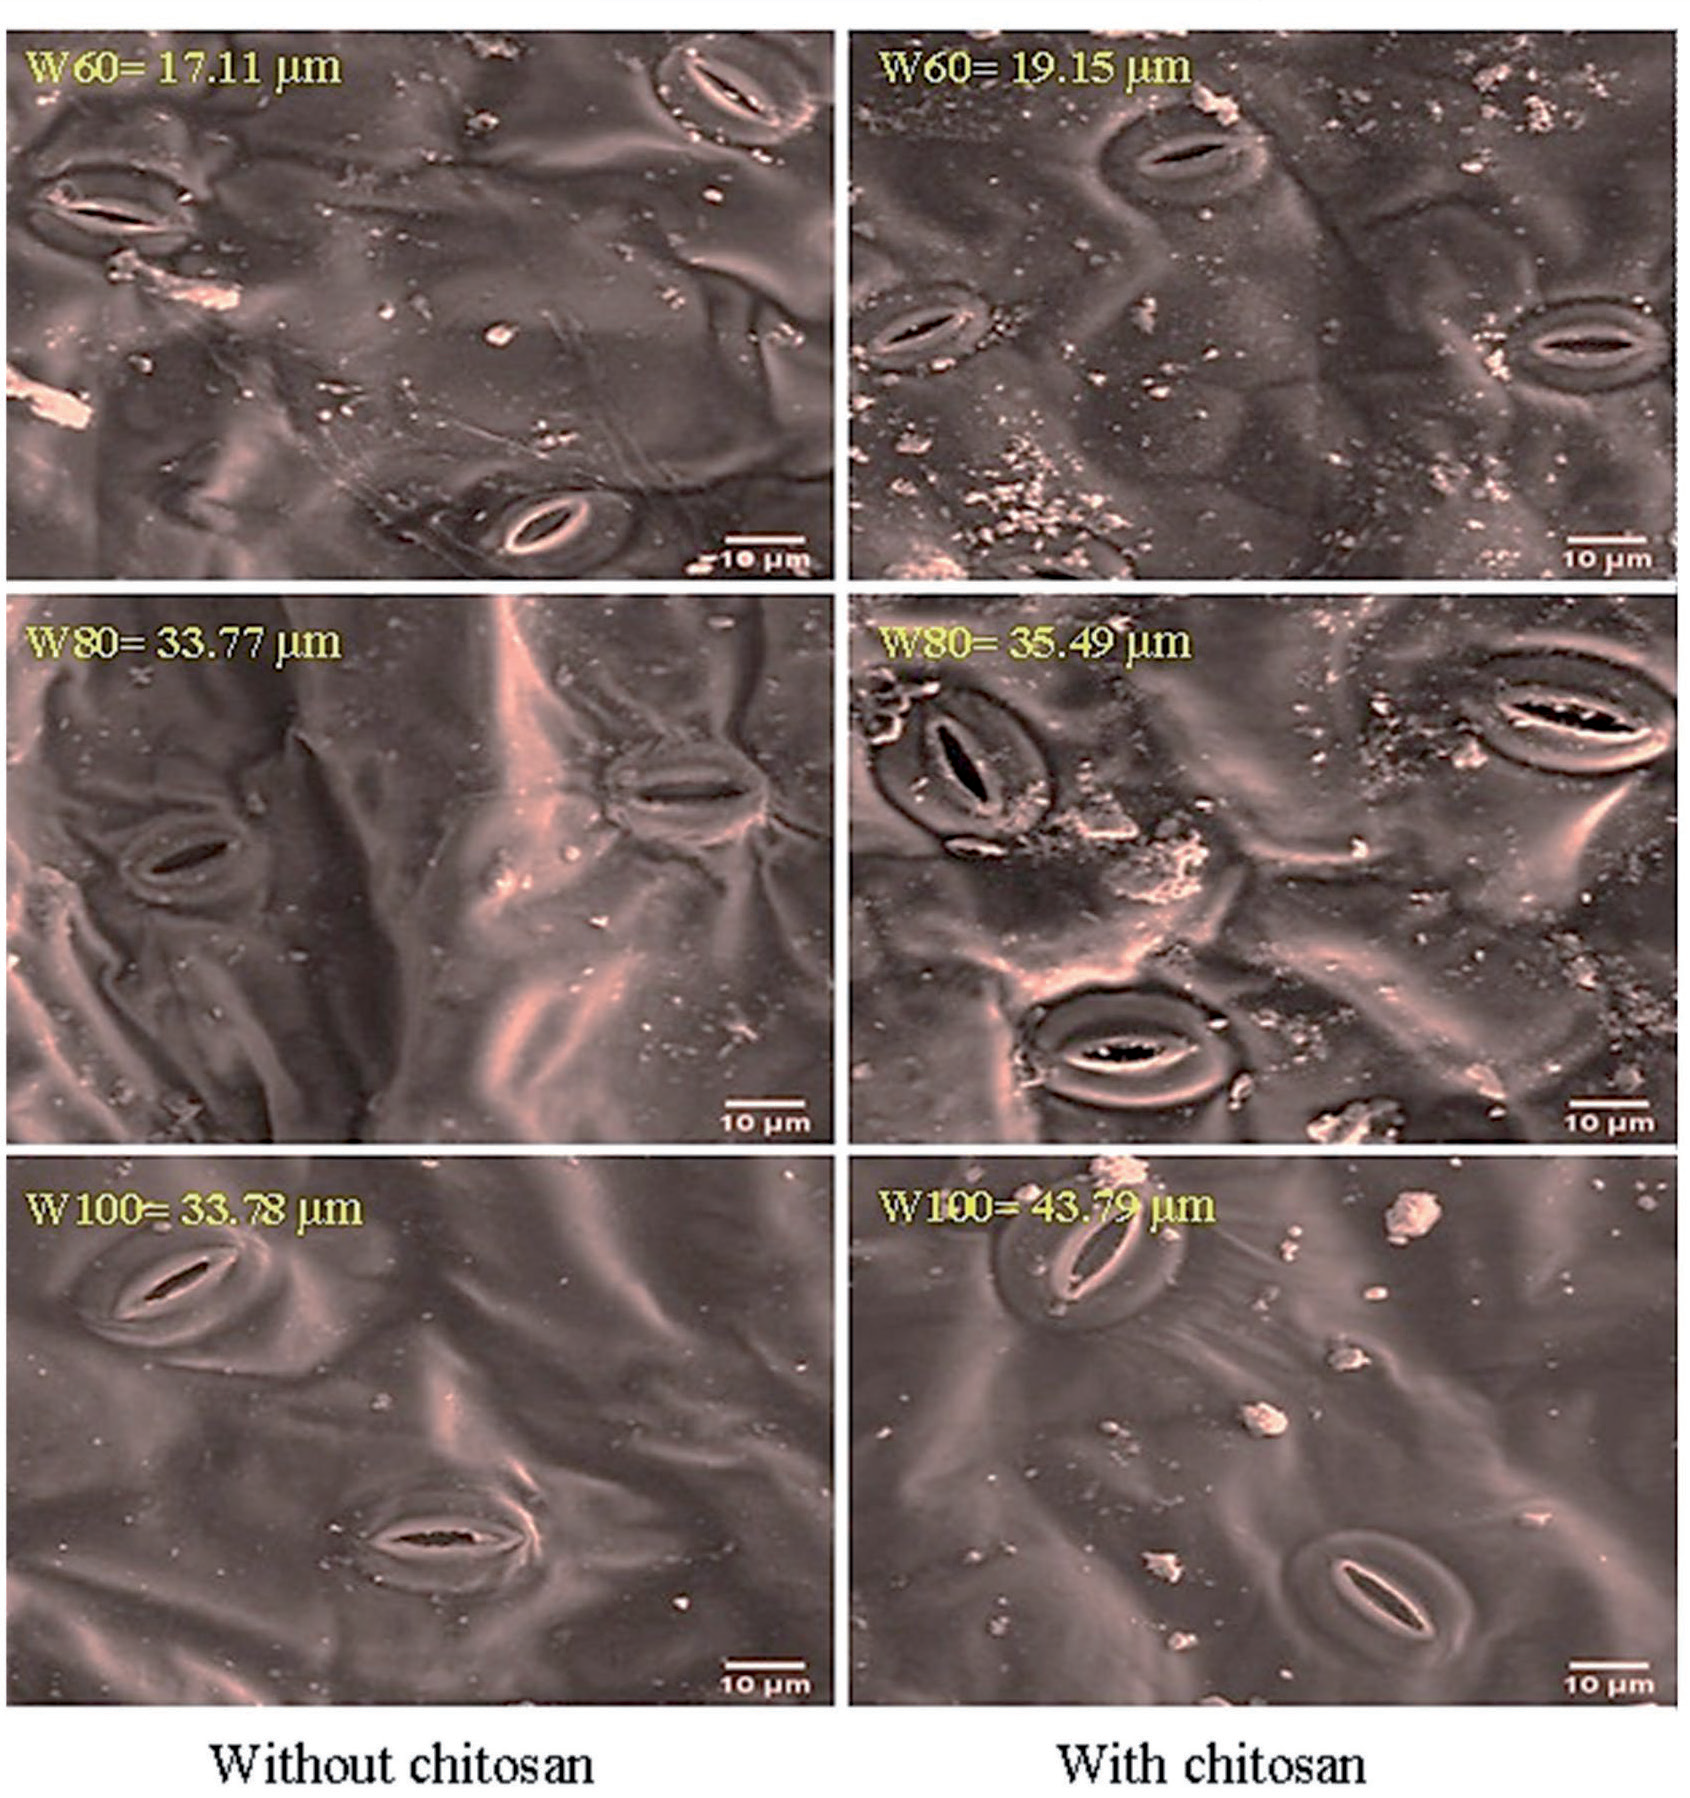
Table 1.
Root fresh weight, top fresh weight, leaf area, photosynthetic pigments and root yield of sugar beet as influenced by irrigation level and chitosan application.
Table 2.
Impurities, sugar lost to molasses, extracted sugar and sugar yield of sugar beet as influenced by irrigation level and chitosan application.
Quality of Sugary Juice and Sugar Products
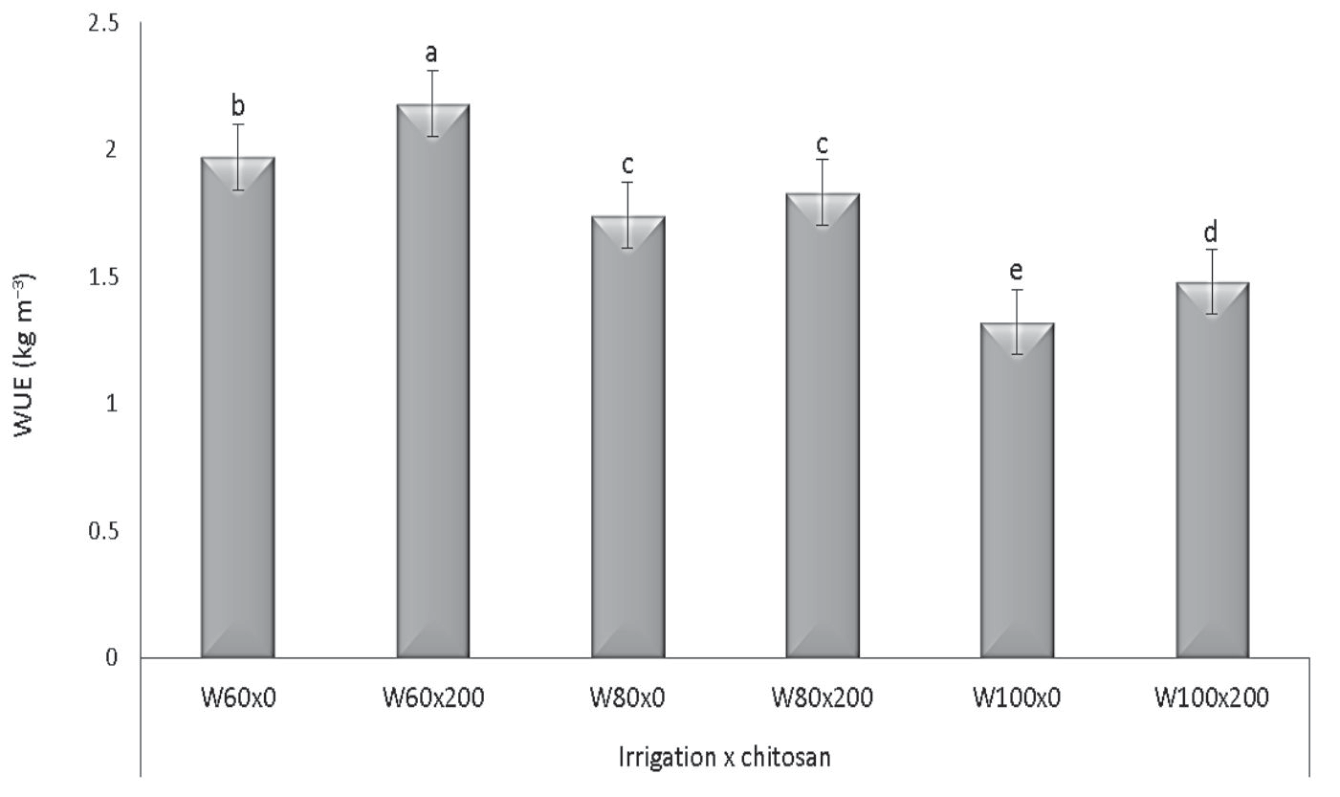
Under W60, chitosan achieved substantial reductions in potassium and sodium, which amounted to 2.6 and 8.0% W, respectively, while increasing the extracted sugar and sugar yield by 5.5 and 10.7%, respectively, compared to no chitosan (Table 2). Moreover, reductions in potassium, alfa amino N, and lost sugar in molasses reached 2.5, 24.4, and 4.7%, respectively, owing to chitosan application under well-watered conditions (W100). On the other hand, the increases in extracted sugar and sugar yield due to chitosan spraying were 7.4 and 12.1%, respectively, under W100. Improvements in sugar beet yield under reduced water supplies due to the use of chitosan also improved water use efficiency (Fig. 4). Under different irrigation levels, plants receiving chitosan solution spray recorded high water use efficiency [45].
Water Use Efficiency
A remarkable interactional influence of irrigation level and chitosan application on the water use efficiency of sugar beet was observed (Fig. 4). Generally, the most efficient combination for enhancing water use efficiency in sugar beet was W60 x chitosan, surpassing the other combinations. Under irrigation by W60 and W100, chitosan caused increases in the water use efficiency of sugar beets that amounted to 10.7 and 12.1%, respectively, compared to no chitosan application.
Fig. 4.
Water use efficiency (WUE) of sugar beet as influenced by irrigation level and chitosan (mg L−1) application. W60, W80 and W100: irrigation by 60, 80 and 100% of crop evapotranspiration, respectively. Values are the mean of 3 replicates ± standard errors. Varied letters within bars signalize that there are significant differences by Duncan’s Multiple Range Test at p≤0.05
Irrigation level had a significant effect on nutrient uptake, soil organic matter, and soil activity, thereby changing plant nutrient constituents [46, 47]. The findings of this study clarified that severe drought stress (W60) increased sugar impurities (alfa amino N and K) as well as the extracted sugars, which were greater than those that were well–watered (W100). Drought caused a reduction in root moisture content; hence, sugar content increased [48]. Additionally, sucrose and hexose sugars have the potential to regulate stress–correlated gene expression engaged in the photosynthesis process, sucrose metabolism, and the synthesis of osmolytes [49-51]. This led to an improvement in the percentage of sugar [52]. Likewise, the alfa amino N group plays a crucial role in the synthesis of various free amino acids like proline and glycine betaine, which have significant potential to conserve moisture in cells, raising sugar lost to molasses [53]. Our results emphasized the favorable action of chitosan in lowering the impurities and treacle sugar, with an increasing sugar percentage and yield (Table 2). In this regard, Dowom et al. [54] demonstrated that chitosan can regulate sugar metabolism.
Conclusions
Disturbances in sugar beet enzymatic activity, stomata performance, and consequently yield and quality occurred due to providing sugar beet plants with irrigation water amounts that were less than normal. The adverse effects generated by cultivating sugar beet in areas with water shortages could be faced by carboxymethyl chitosan. Chitosan enhanced the enzymatic and non-enzymatic antioxidant-based defense mechanisms to promote reactive oxygen species scavenging activities and modulated the stomata opening and pore area in favor of crop growth under drought. In conclusion, for maintaining sugar beet yield and quality while improving water use efficiency in dry land environments, carboxymethyl chitosan (200 mg L−1) application is considered a safe, clean, and cheap practice in this situation.

