

Introduction
The rhizosphere, a microregion a few millimeters from the surface of the root axis, serves as a unique area where the plant root system interacts with the soil microbial community [1]. These interactions between rhizosphere microbes and the plant root system ultimately determine nutrient uptake, resource cycling, and plant health [2]. Rhizosphere microorganisms inhabit the rhizosphere soil of various plant species, playing a pivotal role in plant growth [3]. Specifically, rhizosphere soil fungi are important decomposers that regulate plant nutrient uptake; thereby, promoting growth and development, enhancing host plant disease resistance, and maintaining microecosystem balance within the rhizosphere.
Soil fungal community diversity maintains soil productivity and is an important indicator for evaluating the stability, health, and sustainability of soil ecosystems [4]. Previous studies have demonstrated that changes in the soil environment can considerably affect the composition of soil fungal communities [5-7]. Additionally, plant community succession can indirectly affect the soil environment, thereby altering fungal composition [8]. In monospecific plantation forests, the forest age is a significant factor influencing changes in soil fungal communities [9]. For example, Wang et al. [10] revealed that the development of Pinus tabuliformis plantation forests altered the soil nutrient content in rhizosphere soil, indirectly affecting rhizosphere fungal composition and diversity. Moreover, Zhang et al. [11] identified that the cycling and allocation capacity of soil elements also change significantly with stand age, further affecting fungal community structure. However, fungal species are specific and complex and respond differently to different soil environments even within the same ecosystem [12]. Determining soil microbial community dynamics that reflect changes in forest age and soil properties is important when assessing interactions between above- and below-ground communities [13]. Therefore, it is necessary to understand the changes in soil fungal communities during the development of plantation forests and to identify the main factors affecting these changes.
Platycladus orientalis, commonly known as lateral cypress and incense cedar, is an evergreen tree in the Cupressaceae family. It is widely distributed in China, with favorable characteristics, such as a well-developed root system, drought and barrenness tolerance, a long growth cycle, and the ability to maintain strong forest stability. Therefore, its seedlings are preferred for the afforestation of barren mountains, playing a key role in artificial vegetation construction [14]. The rhizosphere soil microenvironment of P. orientalis may undergo changes with forest age, which could potentially affect the interactions between rhizosphere microorganisms and lateral cypress. Therefore, the present study investigates the soil environment and soil fungal community structure of P. orientalis plantation forests of different ages in Jungar Banner, China. Specifically, we aimed to explore the rhizosphere soil environment and community diversity of P. orientalis plantation forests across different stand ages and to determine the correlations between rhizosphere soil and soil fungal community succession during the development of P. orientalis plantation forests.
Materials and Methods
Study Site
The study site was located in Jungar Banner (110°05′- 111°27′E, 39°16′-40°20′N), Ordos City, Inner Mongolia Autonomous Region, China (Fig. 1). The study site receives average annual sunlight, temperature, and precipitation of over 3,000 h, 6.2–8.7 ℃, and 400 mm, respectively. The soil types present in the study area include chestnut, calcium, and windy sandy soils. P. orientalis has been planted extensively for over 40 years in the study area, and many planted P. orientalis forests of different ages have been created through effective management practices. The study area has sparse herbaceous plants, with dominant Puccinellia tenuiflora and Leymus chinensis species.
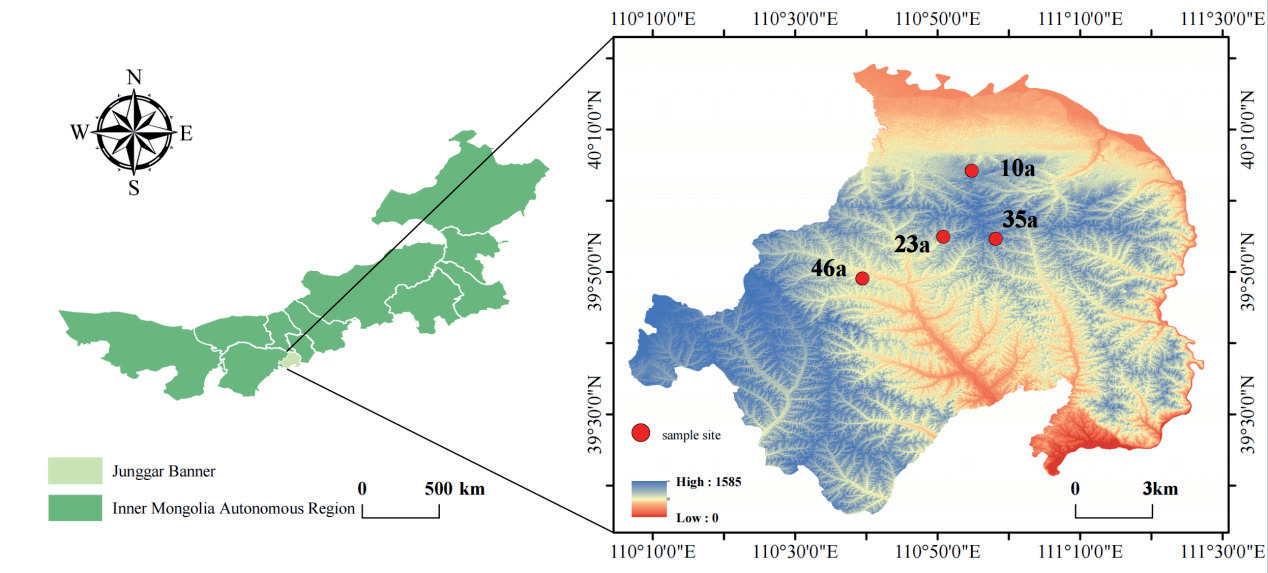
Table 1.
Sampling plot details.
Soil Sample Collection and Analysis
In August 2024, we utilized the spatiotemporal intergenerational method to investigate forest stands in the area. Stands under similar conditions, including management style, slope, slope direction, and soil type, were selected to avoid introducing variation due to differences in ecological conditions. We identified four ages of P. orientalis plantations based on records from the local forestry department: 10 years old (10a), 23 years old (23a), 35 years old (35a), and 46 years old (46a). Detailed information is provided in Table 1. Three plants of P. orientalis (growth condition, diameter at breast height were similar) were randomly selected in the sample plots of each forest age, and within 1 meter from the trunks of the trees, a 0-30 cm soil profile was dug, and roots with fine roots were taken from near the main root system, the large pieces of soil attached to the roots were shaken off, and the soil adhering to the fine roots was collected into self-sealing bags with a sterile brush. The soil from the 4 directions was thoroughly mixed to obtain this P. orientalis rhizosphere soil sample, and a total of 12 soil samples were obtained. The soil samples were halved, and one half was placed into a sterile self-sealing bag and stored at -80 ℃ for DNA extraction. The other half was air-dried and passed through a 2-mm sieve for soil chemical analysis.
Total nitrogen (TN) and effective N were determined by the Kjeldahl method [15] and NaOH alkaline diffusion method [16], respectively, and soil effective N included available nitrogen (AN) and nitrate nitrogen (NN). Total phosphorus (TP) and available phosphorus (AP) were determined by NaHCO3 leaching-molybdenum-antimony resistivity [17]; total potassium (TK) was determined by NaOH melting-molybdenum-antimony resistivity [18]; available potassium (AK) was determined by NH4OAc leaching-flame photometry [19]; soil organic matter (SOM) by K2Cr2O7 oxidation [20]; and soil pH by pH meter.
DNA Extraction and High-Throughput Sequencing
We employed the ITS1F (5′-GGAAGTAAAAGTCGTAACAAGG-3′) and ITS2R (5′-GCTGCGTTCTTCATCGATGC-3) primers for the amplification of the fungal ITS1-ITS2 region. The polymerase chain reaction (PCR) system comprised 25 µL of reaction buffer (5 µL [Thermo Fisher Scientific]), GC high-fidelity buffer (5 µL [Thermo Fisher Scientific]), Q5DNA polymerase (0.25 µL), deoxynucleotide triphosphate (10 µM, 2 µL), and double-distilled H2O (8.75 µL). PCR cycling program was performed as follows: pre-denaturation at 98 °C for 5 min, followed by 30 cycles of denaturation at 98 °C for 30 s, annealing at 55 °C for 45 s, and extension at 72 °C for 45 s. Subsequently, the separation of PCR products by gel electrophoresis was performed. Then, target fragments were excised and recovered using the Axygen Gel Recovery Kit (Thermo Fisher Scientific). The Shanghai Personalbio Technology Co., Ltd., Shanghai, China, performed Illumina MiSeq sequencing analysis.
Data Preprocessing and Bioinformatics Analysis
The raw sequencing data were processed using QIIME2 software (Jacobs School of Engineering, La Jolla, CA, USA). First, the cutadapt plug-in (Jacobs School of Engineering) was used for primer excision. Next, quality control, denoising, removal of low-quality sequences and chimeras, amplicon sequence variant clustering with 100% similarity, and comparative annotation against the Greengenes database were performed using the DADA2 plug-in (Jacobs School of Engineering). Alpha diversity indices were calculated using QIIME2 software (Jacobs School of Engineering). Subsequently, samples were analyzed using linear discriminant analysis based on taxonomic composition under different grouping conditions using Lefse software (Huttenhower Lab, Boston, MA, USA). Functional classification of each sequence, including trophic mode and growth status, was annotated using the FUNGuild online database (http://github.com/ UMNFuN/FUNGuild).
Data Analysis
Significance differences were evaluated using SPSS 22.0 software (SPSS, Chicago, IL, USA). The soil fungal community alpha diversity index was analyzed using Mothur software (National Institutes of Health, Bethesda, MD, USA). Additionally, the similarity in soil fungal community abundance at different forest ages was assessed using cluster analysis in the Vegan program package (https://cran.r-project.org/web/pac kages/vegan/ index.html) in R software (Version 3.3.1 [RStudio, Boston, MA, USA]). Principal coordinate analysis (PCoA) and distance-based redundancy analysis (db-RDA) were performed to explore community structure. Furthermore, structural equation modeling (SEM) was performed using AMOS software (Version 20.0, Amos Development Corporation, Meadville, PA, USA). One-way analysis of variance was employed to identify significant correlations between forest age and soil physicochemical properties and fungal alpha diversity.
Results
Soil Properties
The physicochemical properties of the rhizosphere soil in P. orientalis plantation forests exhibited significant changes with increasing forest age (Table 2). Specifically, results revealed that increasing forest age significantly (p<0.05) increased the TN, NN, AN, TK, and SOM contents in the rhizosphere soil. Contrastingly, the TP content significantly decreased; whereas, AP initially increased and then decreased, reaching its peak in the 35a forest stand. In addition, no significant correlation between rhizosphere soil pH and stand age in P. orientalis.
General Characterization of Rhizosphere Fungal Communities
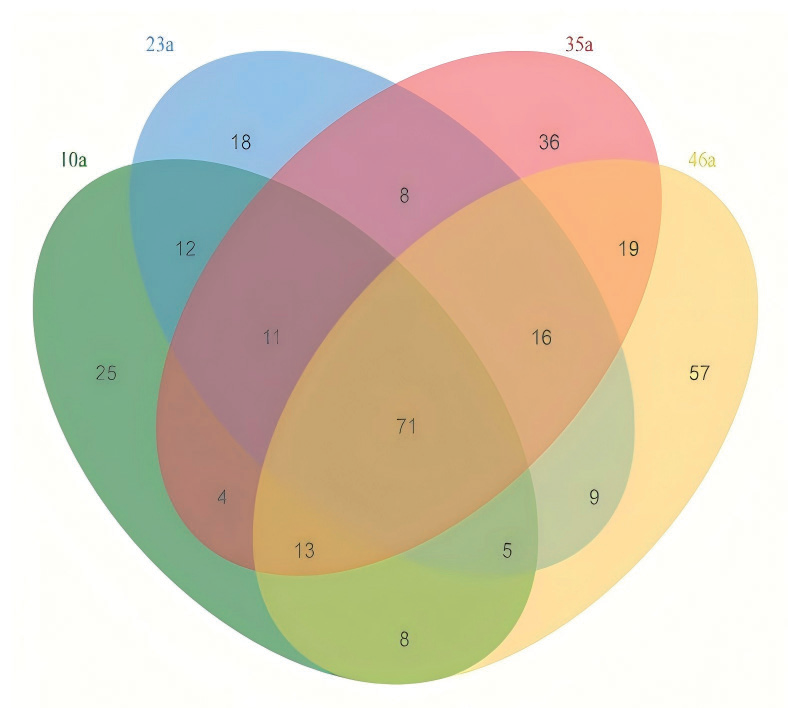
Illumina MiSeq sequencing revealed 690,400 fungal sequences, which were classified into 740 operational taxonomic units (OTUs). Among these, 385 OTUs were identified at the genus level, distributed across 9 phyla, 38 classes, 89 orders, 213 families, and 312 genera. Rhizosphere soil samples from 10a, 23a, 35a, and 46a P. orientalis plantations contained 149, 150, 178, and 198 fungal genera, respectively (Fig. 2). Among these genera, 71 were shared across the 4 forest ages. Additionally, the rhizosphere soil samples from 10a, 23a, 35a, and 46a P. orientalis plantations contained 25, 18, 36, and 57 endemic genera of fungi, respectively.
Table 2.
Soil properties of Platycladus orientalis across different stand ages.
[i] Note: Data are expressed as mean ± standard deviation. Different lowercase letters indicate significant differences at p < 0.05 level of significance based on analysis of variance. NS: Non-significant regressions along the chronosequence; *: p < 0.05; **: P < 0.01. AN-available nitrogen, TN-total nitrogen, NN-nitrate nitrogen, TP-total phosphorus, AP-available phosphorus, TK-total potassium, AK-available potassium, SOM-soil organic matter.
Fungal Diversity and Structure
The results of the diversity analysis showed that forest age significantly affected the Chao1 and Pielou's evenness indices (p < 0.05) but had no significant effect on the Shannon and Simpson indices (p > 0.05) (Table 3). Diversity indices showed a trend of first increasing and then decreasing with forest age. Among these, the Chao1 index of soil fungi at 35a was significantly higher than that of the other three forest ages (p < 0.05); the Pielou index of soil fungi at 23a and 35a was significantly higher than that at 46a (p < 0.05); the Shannon index of soil fungi at 35a was significantly higher than that at 46a (p < 0.05), while the Simpson index of soil fungi at 46a was significantly lower than that of the other three forest ages (p < 0.05).
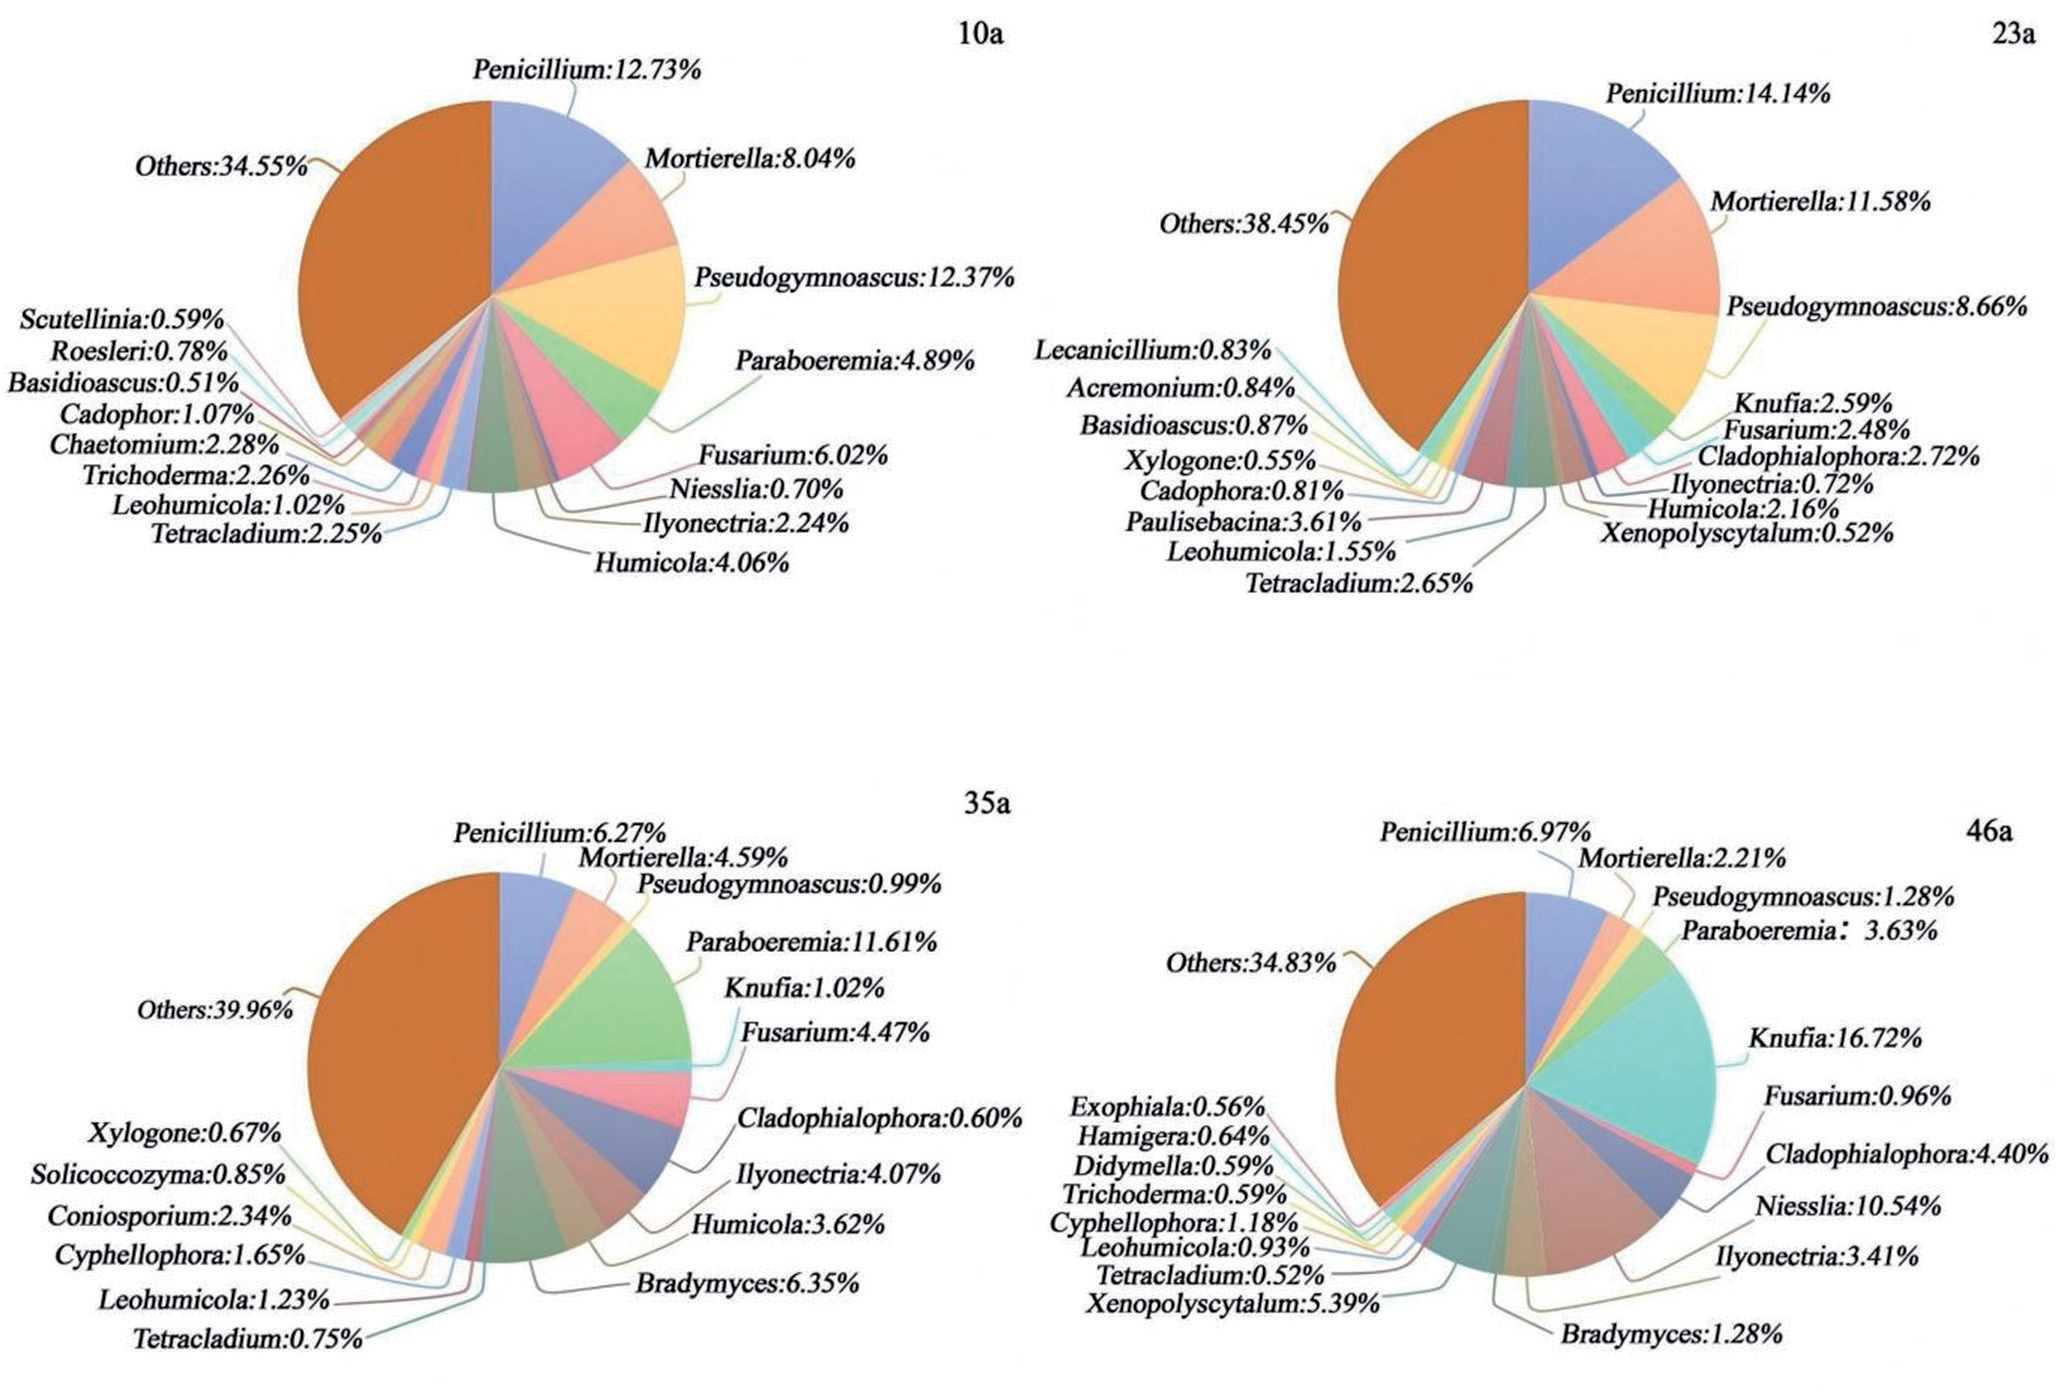
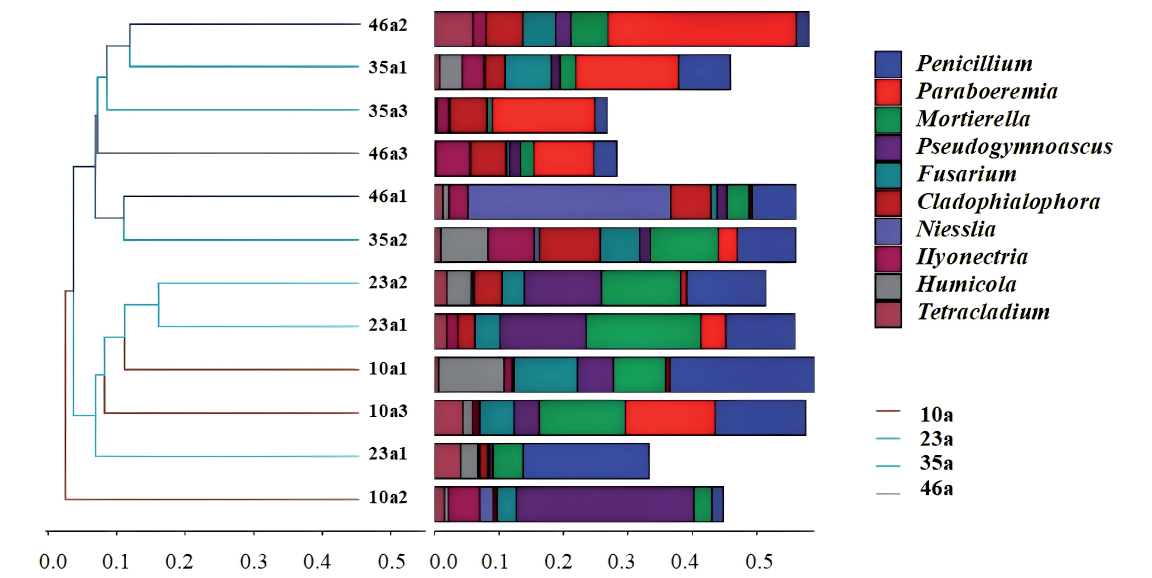
Significant differences in the rhizosphere soil fungi at the phylum level were observed in P. orientalis plantation forests of varying stand ages (Fig. 3). The abundance of soil fungi from the phyla Basidiomycota and Mortierellomycota increased initially and then declined with increasing stand age of P. orientalis plantations, reaching their highest levels in the 23a stand. Conversely, the Ascomycota abundance decreased initially and then increased, reaching its peak in the 46a stand. Furthermore, soil fungi from P. orientalis plantation forests of varying stand ages differed significantly (p < 0.05) at the genus level (Fig. 4). Penicillium, Pseudogymnoascus, and Mortierella were the top three dominant genera in the 10a stand considering relative abundance. In the 23a stand, Penicillium, Mortierella, and Pseudogymnoascus were the dominant genera; whereas, Paraboeremia, Bradymyces, and Penicillium were dominant in the 35a age stand. In the 46a stand, Knufia, Niesslia, and Penicillium were the dominant genera. Penicillium was distributed in four forest stands and had a relatively high relative abundance.
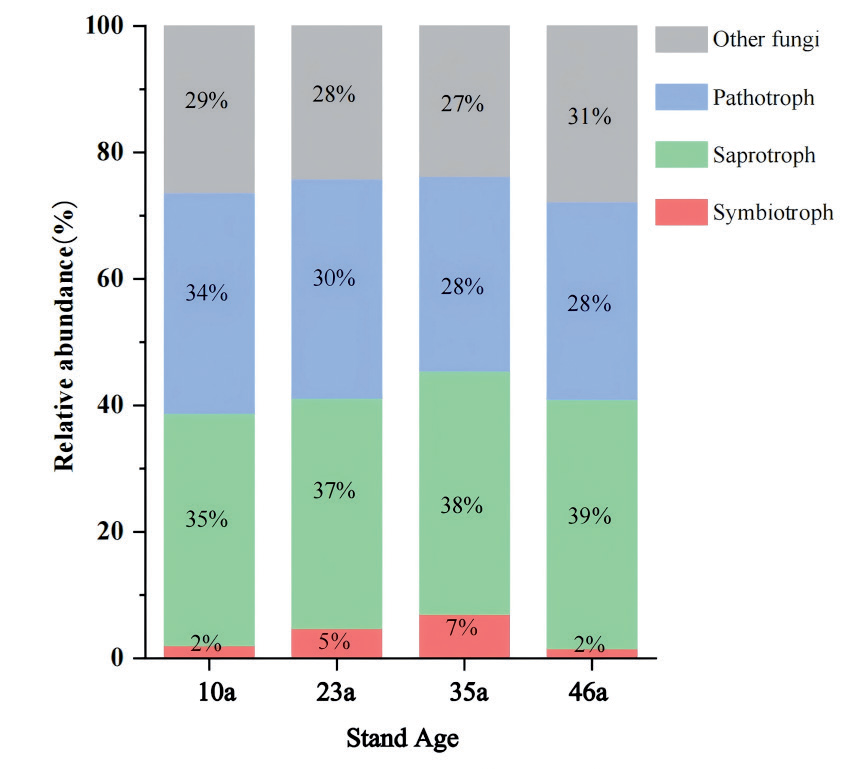
The functional classification annotation results demonstrated that the rhizosphere soil fungi of P. orientalis plantations predominantly exhibited three trophic types: pathotrophs, symbiotrophs, and saprotrophs (Fig. 5). The proportions of these functional groups varied significantly across different forest ages. Specifically, as forest age increased, the relative abundance of pathotrophs gradually increased and then stabilized. Meanwhile, the saprotrophs exhibited a gradual increase, and symbiotrophs initially increased and decreased, reaching their peak at 35a. Additionally, a higher relative abundance of fungi not identified as functional taxa was observed in the soil of the 46a stand than in the soil of the other stand ages.
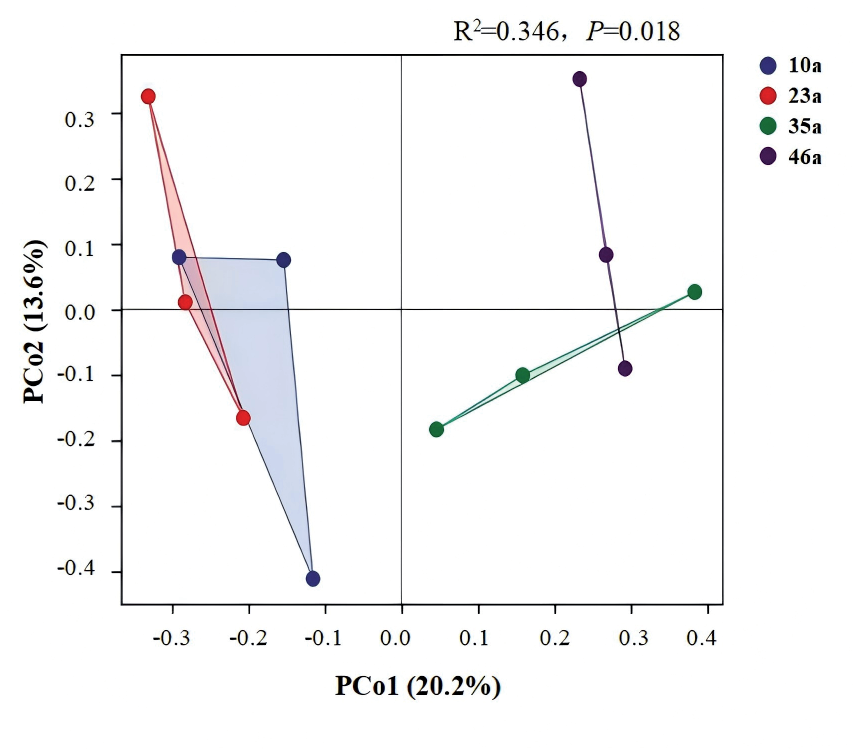
The PCoA results revealed significant differences in the rhizosphere soil community composition across different stand ages of P. orientalis plantation forests (R2 = 0.346, p = 0.018) (Fig. 6). Notably, the soil fungal communities of the 10a and 23a stands were notably distant from those of the 35a and 46a stands in the PCoA results. Contrastingly, the soil fungal communities between the 10a and 23a, and those between the 35a and 46a stands, were in close proximity, indicating a greater similarity in their community compositions. Furthermore, Hierarchical cluster analyses also showed more similarity in soil fungal community structure between the 10a and 23a stands, and great similarity between 35a and 46a stands (Fig. 7). The differences in the soil fungal composition among P. orientalis plantation forests of different stand ages primarily presented as changes in the relative abundances of Paraboeremia, Mortierella, Pseudogymnoascus, and Niesslia.
Table 3.
Diversity index of rhizosphere soil fungi associated with Platycladus orientalis plantation forests at different stand ages.
Fig. 3.
Composition of soil fungal communities at the phylum level across different stand ages of Platycladus orientalis plantation forests.
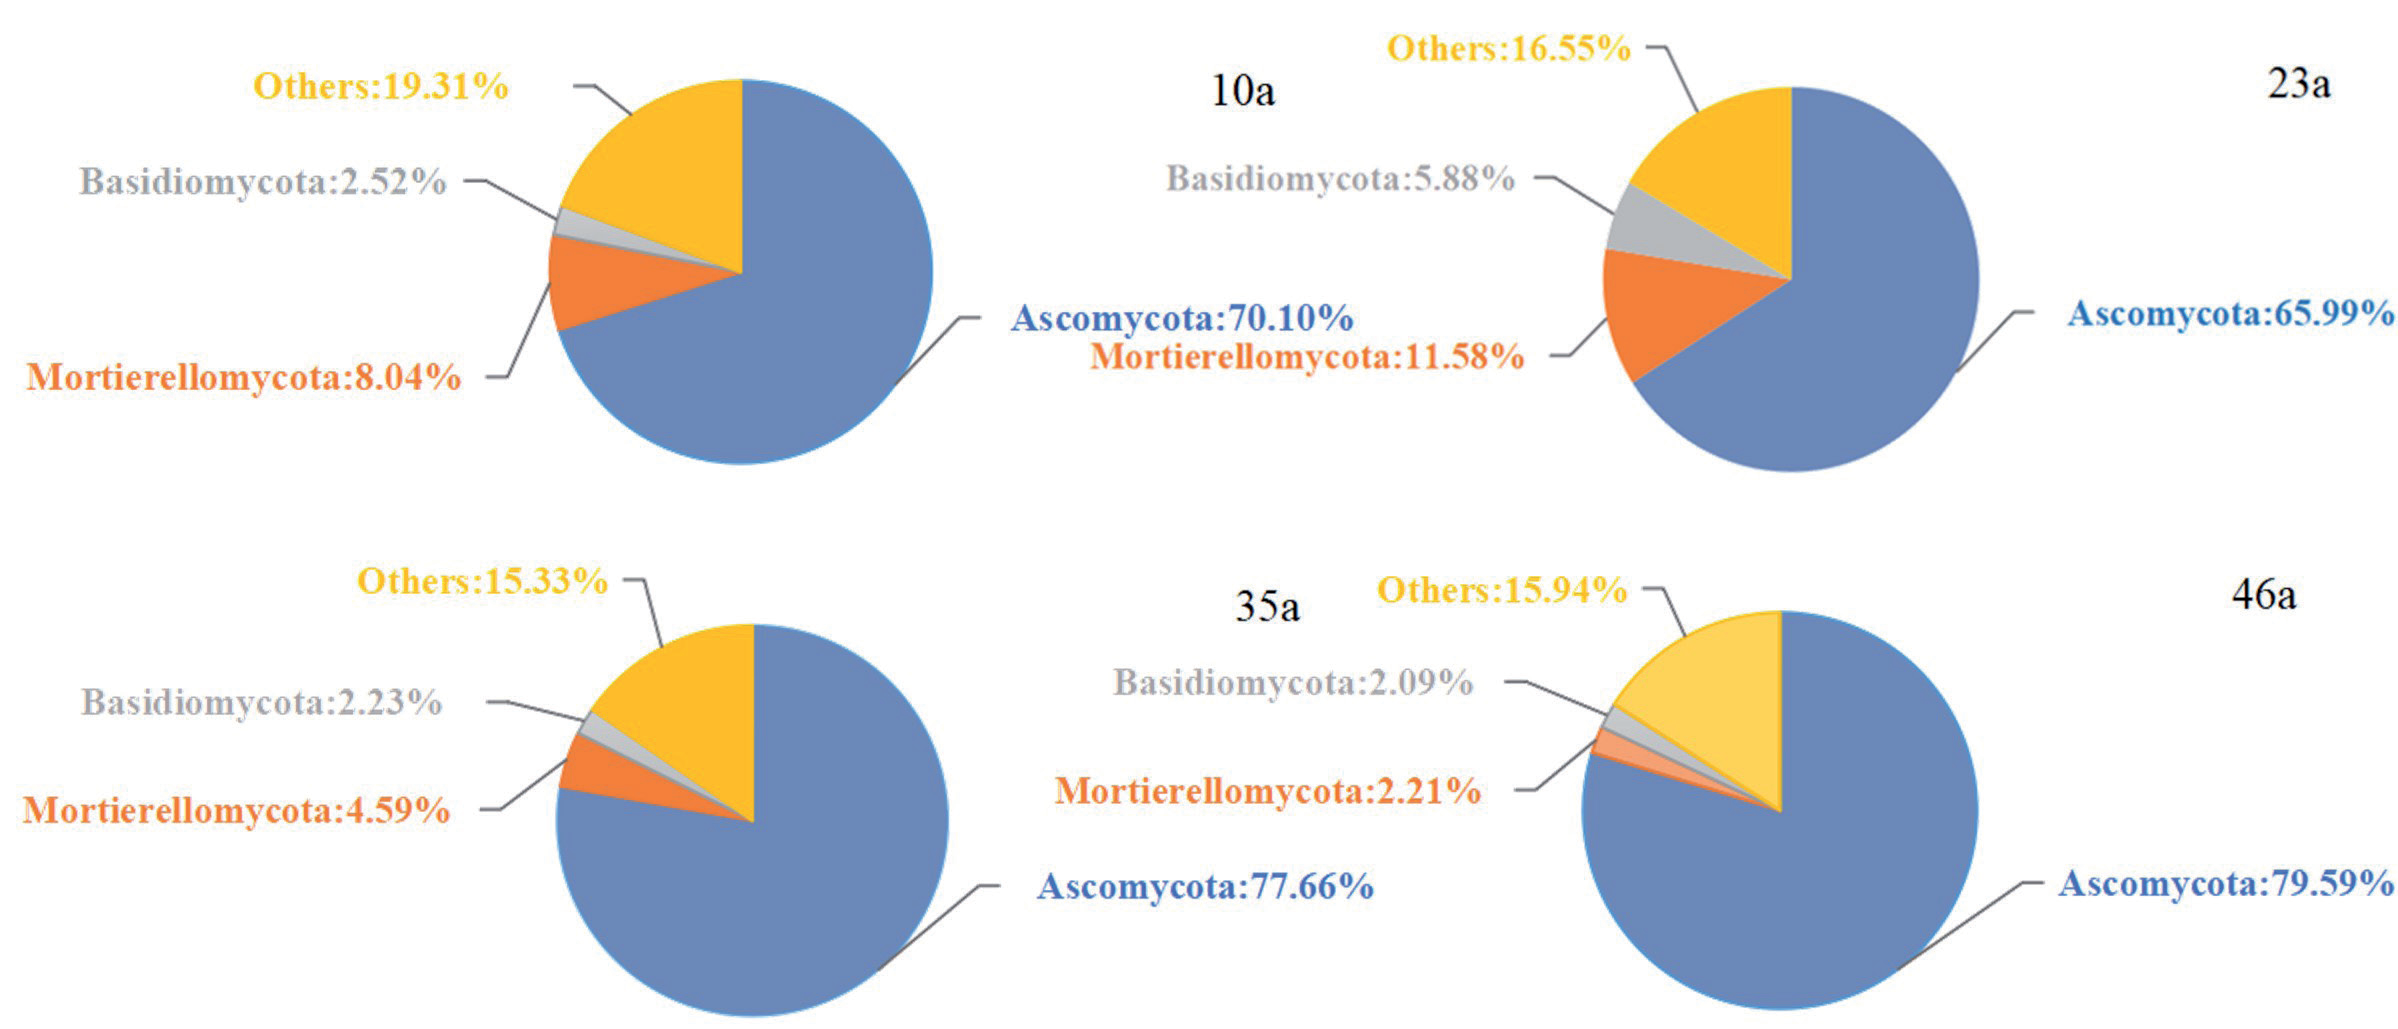
Fig. 4.
Composition of soil fungal communities at the genus level across different stand ages of Platycladus orientalis plantation forests.
Correlation Among Fungal Community Composition and Soil Nutrients
The db-RDA results showed that there were relationships between the distribution of rhizosphere soil fungal communities and soil physicochemical properties across different stand ages of P. orientalis plantation forests (Fig. 8). The first principal axis accounted for 18.3% of the variance, with the first and second explanatory axes jointly accounting for 30%. Notably, TP content (p < 0.01), pH (p < 0.01), and NN content (p < 0.05) significantly influenced soil fungal communities. The results of correlation analysis showed that soil fungal genera were significantly correlated with soil physicochemical properties at different forest ages (Fig. 9). The relative abundance of Penicillium, Roesleria, and Fusarium showed significant positive correlation with soil pH (p < 0.05), Humicola showed highly significant positive correlation with soil pH (p < 0.01), Xenopolyscytalum and Exophiala showed significant negative correlation with pH (p < 0.05); Cadophora and Tetracladium were significantly positively correlated with TP content (p < 0.05), Cladophialophora and Cyphellophora were significantly negatively correlated with TP content (p < 0.05); Fusarium and Cladophialophora were significantly positively correlated with the content of TN and NN (p < 0.05); Scutellinia showed significant positive correlation with soil TN (p < 0.05); Pseudogymnoascus and Cadophora were significantly negatively correlated with NN content (p < 0.05).
Fig. 6.
Principal coordinates analysis of soil fungal communities in Platycladus orientalis plantation forests across different stand ages.
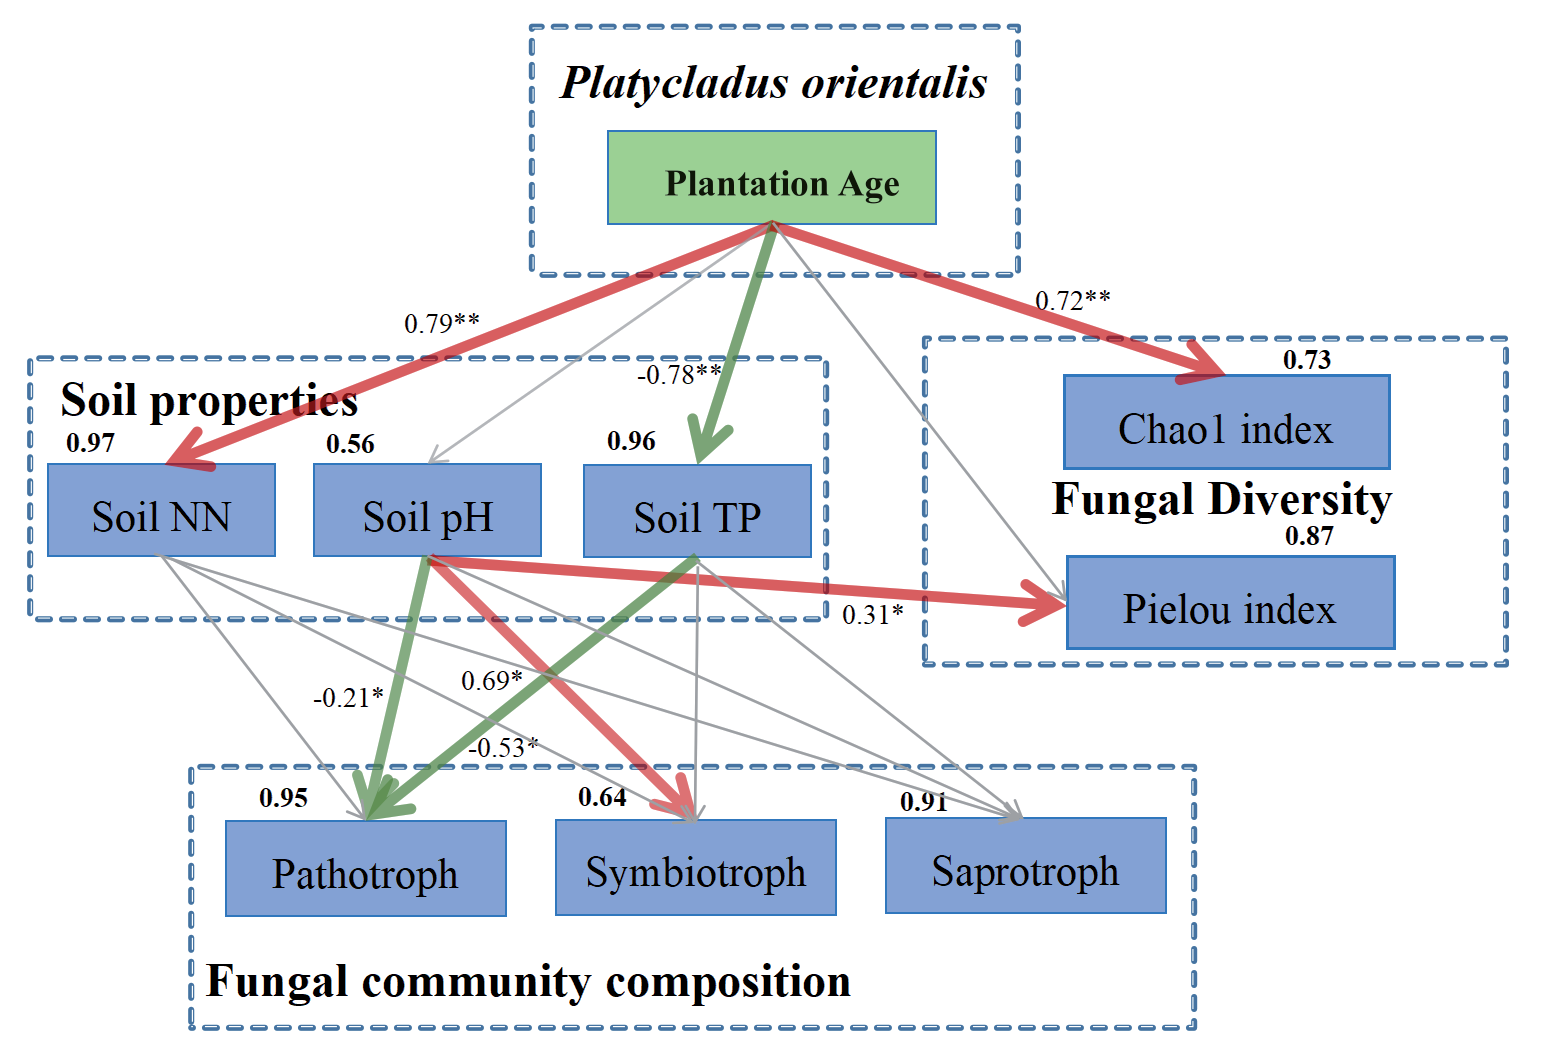
Finally, the SEM results showed that increasing stand age significantly increased soil NN content and Chao 1 index diversity while reducing TP content (Fig. 10). Additionally, an increase in pH and TP content significantly decreased the relative abundance of pathotrophs, while the increase in pH also significantly increased the relative abundance of symbiotrophs and the Pielou index.
Fig. 9.
Correlation analysis between soil fungal community composition and soil properties in Platycladus orientalis plantation forests. *: p < 0.05, **: p < 0.01.
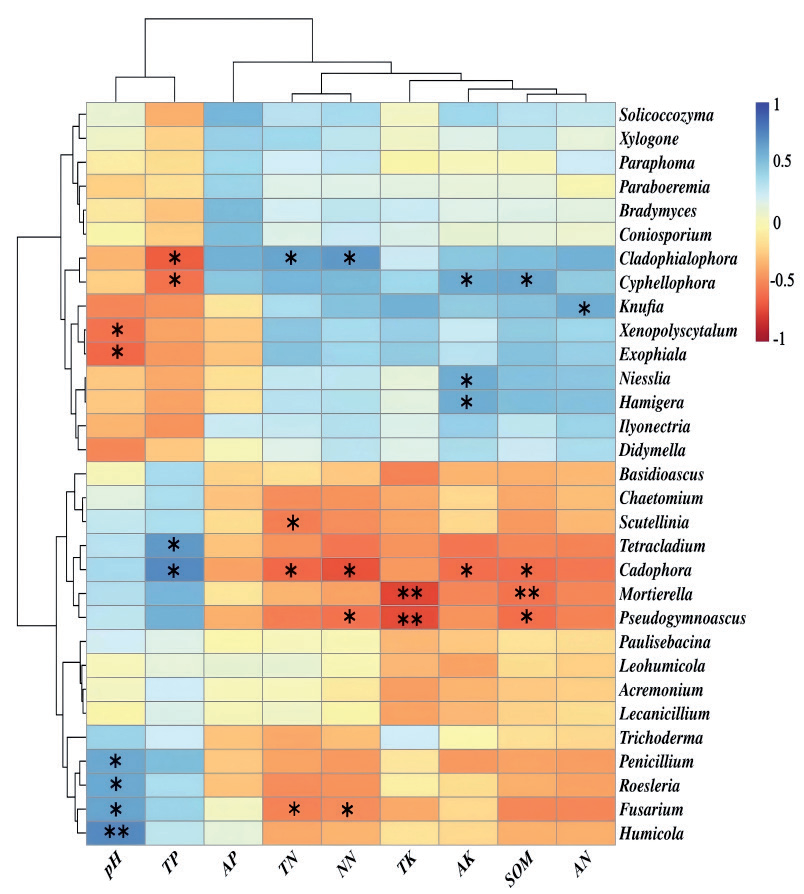
Fig. 8.
Distance-based redundancy analysis of the soil fungal community structure in Platycladus orientalis plantation forests across different stand ages.
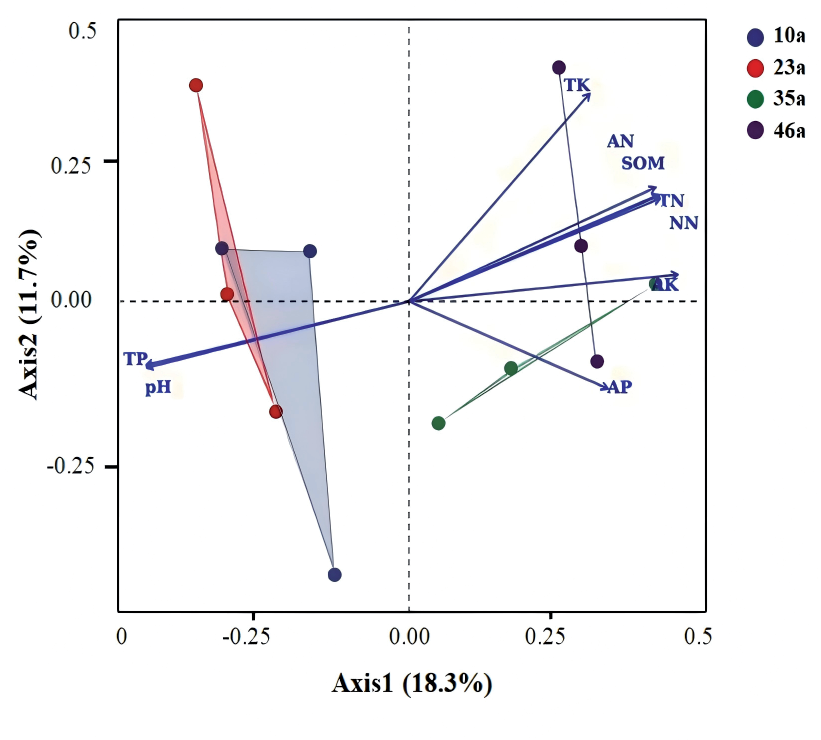
Fig. 10.
Structural equation model of plantation age, soil physicochemical properties, and soil fungal community composition and diversity in Platycladus orientalis plantation forests. The numbers provided for each component in the model reflect the coefficient of determination R2; meanwhile, the numbers adjacent to the arrows indicate the path coefficients. Red, green, and gray arrows represent positive, negative, and no significant correlations, respectively. NN: nitrate nitrogen, TP: total phosphorus. *: p < 0.05, **: p < 0.01.
Discussion
The compositional structure of forest ecosystems, internal environment, and soil physicochemical properties have been found to change with increasing forest age. The present study revealed that soil AN, TN, NN, TK, and SOM contents increased with increasing age of P. orientalis. As the age of P. orientalis forests increases, the amount of litter under the canopy also increases. Litter on the ground is decomposed by microorganisms and root secretions and converted into organic nutrients [21-22]. Soil SOM and N elements mainly come from ground litter, resulting in a continuous increase in AN, NN, TN, and SOM content in the soil. The primary means by which soil acquires P comes from the weathering of rocks and leaching, and the method of acquisition is relatively singular [23]. Soil TP content decreased with increasing stand age; whereas, AP content initially increased and then decreased. TP content significantly decreased between 23a and 35a, but AP content increased significantly during this period. However, although the TP content in the soil of the 35a stand was low, conducive soil conditions contributed to the release of P from apoplast or soil minerals, ultimately increasing AP content and enhancing plant growth. Therefore, P. orientalis plantation succession ameliorates P deficiency in plants in the study area [24]. However, the soil TP contents of 35a and 46a stands were 0.73 g/kg and 0.52 g/kg, respectively, which is considered severely phosphorus-deficient soil. Furthermore, the study area had no supplementation of the P element by weathering of mineral rocks. Therefore, ecosystem management in Jungar Banner P. orientalis plantation forests should focus on increasing P content in the soil to meet the future demand for forest productivity.
In this study, the Chao1, Pielou-e, Shannon, and Simpson indices unexceptionally increased with the extension of forest age and decreased subsequently. This is similar to the research findings of Cao et al. [25] on the characteristics of soil fungal communities in Cunninghamia lanceolata forests at dissimilar stages of development. The reason may reside in that as the forest ages, the ecosystem gradually matures throughout the early stages, providing fungi with diverse habitats and resources, ultimately giving rise to an increase in the diversity index. As the ecosystem matures further, certain fungal species may exhibit a downturn trend due to competition, and the community structure may stabilize, resulting in a decline in the diversity index [26]. In addition, both PCoA analysis and hierarchical clustering analysis results suggest that the soil fungal community compositions of the 35a and 46a stands are more similar, which demonstrates that the fungal community in the rhizosphere soil of P. orientalis tends to stabilize as forest age increases. The aforementioned phenomenon illustrates that the underground ecosystem has reached a relatively stable equilibrium. Nonetheless, this study focused attention on 10a to 46a P. orientalis plantation forests. In addition, it is imperative to conduct more profound research on the soil fungal community succession, so as to understand the future succession process of P. orientalis plantation forests.
In this study, Ascomycota, Basidiomycota, and Mortierellomycota were dominant in all forest ages, which is consistent with the results of the study by Xu et al. [27]. It is noteworthy that Ascomycota demonstrated exceptional abundance in all four forest ages, all exceeding 65%. Ascomycota is the dominant fungal phylum globally, occupying the largest proportion of soil fungal species. It plays a paramount role as an important decomposer in soil, thereby contributing tremendously to the degradation of organic matter and soil nutrient cycling [28]. Basidiomycota is a diverse group of fungi that can form symbiotic relationships with plant roots to form mycorrhizae, which contribute to plant stress tolerance. Basidiomycota displays superior degradation capabilities for difficult-to-degrade substances such as cellulose and lignin. Most species of Mortierella within the Mortierellomycota are beneficial to plants [29]. The abundant presence of these three types of fungi can not only heighten the rate of litter decomposition in the soil, ameliorate soil fertility and utilization, but also bring more nutrients for plant growth, and push ahead soil restoration subsequent to afforestation [30]. In this study, there were differences between dominant genera of different forest ages. The dominant genera in the 10a and 20a stands were Penicillium and Mortierella. The dominant genera in the 35a stand were Pseudogymnoascus and Penicillium. The predominant genera in the 40a stand were Knufia and Penicillium. Penicillium was present in all four forest ages. Penicillium is extensively acknowledged for its production of enzymes and antibiotics, and is crucial for biodegradation, nitrogen metabolism, and promoting plant growth. The abundance of Penicillium was higher in 10a and 23a stands, but conspicuously decreased in 35a and 46a stands. The abundance of dominant fungal genera in the soil reveals noticeable fluctuations and succession patterns with the extension of forest age. This phenomenon may be attributable to the disparities in the adaptive capacity of various fungal groups to physicochemical environmental conditions, with changes in understory microenvironmental factors becoming progressively disadvantageous for their growth and reproduction, eventually triggering a reduction in the abundance or replacement by other groups [31].
Soil fungal communities employ various nutritional strategies to adapt to environmental changes. In the present study, the rhizosphere soil fungi of P. orientalis plantation forests were primarily categorized into three groups: pathotrophs, symbiotrophs, and saprotrophs [32]. The relative abundance of saprotrophs was the highest among the four stand ages, aggregating in large numbers in the 46a stand. Notably, in the 46a stand, there was a notable increase in the amount of apoplastic and necrotic tissues, which provided a substantial pool of SOM for saprotrophic fungi. The apoplastic decomposition by saprotrophs resulted in the release of easily accessible carbon sources into the rhizosphere soil environment, resulting in a peak in N and SOM contents, indicating that the decomposition of apoplastic matter by specific fungal taxa became more efficient over time [33, 34]. Ascomycota fungi, which are predominantly saprotrophs, decompose a wide range of difficult-to-degrade substances and are important decomposers of SOM [35]. The results of the present experiment similarly indicated that Ascomycota abundance reached a maximum in stand 46a. Moreover, there are mutual restraints between different trophic fungi, with the large enrichment of symbiotrophs having antagonistic effects on plant pathotrophs; thereby, reducing their colonization and playing a positive role in the development of P. orientalis plantation forests [36].
Results from db-RDA analysis illustrate that soil pH, TP, and NN stand as primary factors influencing soil fungal communities. In detail, soil pH serves as a pivotal indicator of soil acidity or alkalinity. Apart from that, dissimilar fungal species display varying degrees of adaptability to pH conditions. For this reason, soil pH potentially imposes direct influences on the species composition and abundance of fungal communities in the soil [37]. Numerous studies have shown that soil pH is an important driver of fungal community composition [38, 39]. Apart from that, soil pH is not only bound up with multiple genera, but also reveals a conspicuous and positive correlation with the dominant genus Humicola, further demonstrating that soil pH plays a paramount role in altering soil fungal community composition [40, 41]. NN may indirectly influence fungal communities by altering soil microenvironments (e.g., pH or nitrogen form). Some studies have put forth a viewpoint that NN nutrients can inhibit the growth of pathogens (such as Fusarium), potentially through resource competition or activation of plant resistance [42]. Correlation analysis also suggested a striking and negative association between NN and Fusarium. Soil TP is a key nutrient element that can drive fungal community structure by influencing different fungal functional groups. Other investigations have also drawn a conclusion that TP indirectly affects fungal communities by regulating soil pH and organic matter [43].
As suggested by SEM results, forest age has a positive effect on soil NN and TP content and negatively impacts soil pH. Consistent with the results of studies on Pinus sylvestris var and Cunninghamia lanceolata plantations, pH values exhibited a remarkable decline with the increase of forest age [44, 45]. The reason is that as forest age increases, vegetation cover increases, litter decomposition and root exudate accumulation occur, thus giving rise to soil acidification [46]. As the age of the forest increases, the number and activity of ammonia-oxidizing archaea (AOA) in the soil may change accordingly. Associated studies have revealed that AOA in acidic soils have a higher affinity for ammonia and are better suited to surviving in acidic environments [47]. As the acidity of the rhizosphere soil of P. orientalis increases, the activity of AOA gets more dramatic, thereby elevating the production of NN. As trees age, their root systems become more developed, and root exudates and root residues (such as root hairs and fine roots) also add phosphorus to the soil. These root inputs function as one of the paramount sources of phosphorus in the soil [48]. An abatement in soil pH may trigger the binding of phosphorus with elements such as iron and aluminum, thereby elevating the content of available phosphorus in the soil. On top of that, a remarkable and positive correlation was detected between pH and the relative abundance of symbiotrophs, while pH and TP demonstrated a striking and negative correlation with pathotrophs. The relationship between soil pH and fungal community structure is complex, as it may influence fungal growth and activity through both direct and indirect mechanisms. Optimal pH levels may provide more advantageous growth conditions for symbiotic fungi while inhibiting the activity of pathogenic fungi [49]. TP content in soil imposes direct influence on plant growth, development, and health. High TP levels may facilitate plant growth, reinforce plants' resistance to pathogenic fungi, and thereby lessen the relative abundance of pathogenic fungi [50]. As a consequence, we speculate that increasing the soil pH and TP content in this region could not only propel the growth and development of P. orientalis but also lower the abundance of pathotrophs while lessening the abundance of symbiotrophs. It is crucial to figure out these details for strengthening the management of P. orientalis plantation forests.
Conclusions
In this study, the long-term growth of P. orientalis plantation changed rhizosphere soil nutrients as well as fungal community composition. Soil pH, NN, and AP content were the main factors affecting fungal community composition. Among them, pH was significantly positively correlated with the relative abundance of symbiotrophs, and pH and TP content were significantly negatively correlated with the relative abundance of pathotrophs. In conclusion, the results of the present study revealed the relationship between fungal composition and soil properties in P. orientalis plantation forests, and provided a theoretical basis for the management and sustainable development of P. orientalis plantation forests in this region.

