

Introduction
The use of agricultural water has recently received unprecedented attention. The Ministry of Agriculture and Rural Affairs of China, in its documents on agricultural development and the standardization of high-standard farmland construction, has repeatedly emphasized the importance of improving the utilization efficiency of natural precipitation and irrigation water in agriculture [1, 2]. This becomes particularly crucial in arid agricultural regions such as North China, where enhancing water use efficiency (We) is essential [3]. In the field of water-saving agriculture, researchers have recently discovered that, compared with improving irrigation methods and equipment, scientifically controlling irrigation water consumption can achieve goals more directly and effectively. Therefore, in-depth research on deficit irrigation is critical for improving agricultural We and promoting agricultural development in arid regions. Despite the current development of landmark industries and the flourishing development of characteristic agriculture, water scarcity and low We often become bottlenecks, limiting the scale of agricultural production [4-6].
Deficit irrigation is a type of limited water irrigation method that has demonstrated significant effects on water conservation and consumption reduction, and has received increasing attention [6-9]. The theory of deficit irrigation is maturing, but more evidence is required to elucidate its mechanism comprehensively. During the water-critical period, deficit irrigation uses less water than the total transpiration and evaporation of crops. Different plants exhibit varying degrees of tolerance to deficit irrigation, and simulation experiments must be conducted before application to determine deficit gradients [7, 8, 10-14]. Deficit irrigation during the seedling stage can reduce water consumption without reducing crop yield or having a minimal impact on yield, which is crucial for improving water resource utilization efficiency in arid areas [5, 12, 13].
Sunflowers, a significant oil crop, are primarily cultivated in different regions, including Inner Mongolia, Xinjiang, and northeastern China. [9] The climatic conditions in these areas often pose a risk of drought during sunflower cultivation. The actual production of sunflowers has been severely suppressed by limited precipitation and an unevenly distributed climate in major production areas like Inner Mongolia and Xinjiang, as well as the limitations of various resources in China. [3, 9] Research indicates that a water deficit could potentially lead to a 50% reduction in sunflower yield [15]. Consequently, exploring water-saving irrigation techniques during the seedling stage of sunflowers to improve the utilization of agricultural water resources is crucial for mitigating the losses caused by water deficits [16, 17].
Under deficit irrigation conditions, the exogenous application of endogenous plant signaling molecule salicylic acid (SA) has been demonstrated to play a significant role in improving the adaptive response of plants to adverse environmental conditions, particularly in drought tolerance [18-22]. SA positively regulates the growth and development of quinoa, soybean, potato, and strawberry plants under water-deficit conditions, which is crucial for maintaining normal physiological and biochemical metabolism in plants [22-25]. Although the theory of deficit irrigation has matured to some extent, the underlying mechanisms remain unclear.
This study aimed to explore the response of sunflowers to SA and its relationship with proteomics under varying deficit irrigation conditions to provide a theoretical and scientific foundation for water-saving sunflower cultivation techniques in drought-prone areas. Through this series of studies, we aim to provide strong support for improving the national We in agriculture and ensuring food security.
Material and Methods
Test Materials
The experimental plants were selected from the sunflower (Helianthus annuus L.) varieties cultivated in the local arid areas and planted in a greenhouse at the training base of Jining Normal University. A block experiment was conducted with a row spacing of 80 cm, a plant spacing of 50 cm, and a sowing depth of 3 cm. After sowing, consistent management and quantitative irrigation were used to maintain the optimal soil moisture content, which was set at 75% of the field capacity and marked as the control (CK).
Methods
Deficit Irrigation Treatment
A deficit irrigation treatment was initiated upon the development of seedlings to six true leaves. This experiment was designed to assess the impact of varying irrigation levels set at 80%, 60%, and 40% of the CK group watering volume. The irrigation frequency remained consistent throughout the experiment. During the deficit irrigation period, the ring of soil around the root ball of each plant was carefully isolated to ensure individualized watering. SA was sprayed 14 d after the start of the deficit irrigation treatment.
SA processing and indicator determination
The concentration of SA sprayed externally was 20 mg/L, and the SA treatment was applied to all irrigation treatments for comparison with the water spraying. The standard for spraying sunflowers' leaves is to cover their surface with mist droplets without allowing water to drip. When the SA solution dried, leaves with similar heights were cut twice at 0 h and 24 h. The leaves were stored at -80°C, and proteomic analysis was performed. The experiment was conducted by Nucleosome Biotechnology Co., Ltd. (Beijing). Protein identification was performed using Proteome Discoverer 2.5 to simulate protein fragmentation, match theoretical peptide segments, and perform other tasks. The UniProt database was used for protein identification. Functional annotation of proteins was performed using the Cluster of Orthologous Groups of Proteins (COG) database. Differential protein analysis was performed and represented using a Volcano Plot, while differential protein functional enrichment analysis was performed using the Kyoto Encyclopedia of Genes and Genomes (KEGG).
The photosynthetic and transpiration indicators were measured at 24 h. From 9 to 11 am, the Top3051D photosynthesis analyzer was used to analyze sunflowers' leaves, with the measurement object being intact leaves that were close in height to the measured proteomics. The recorded indicators included the net photosynthetic rate (Pn), transpiration rate (Tr), stomatal conductance (Cleaf), intercellular CO2 concentration (CO2in), and We.
Results and Discussion
Effects of SA on Leaf Moisture Content and Photosynthetic Index of Sunflowers under Different Deficient Irrigation Conditions
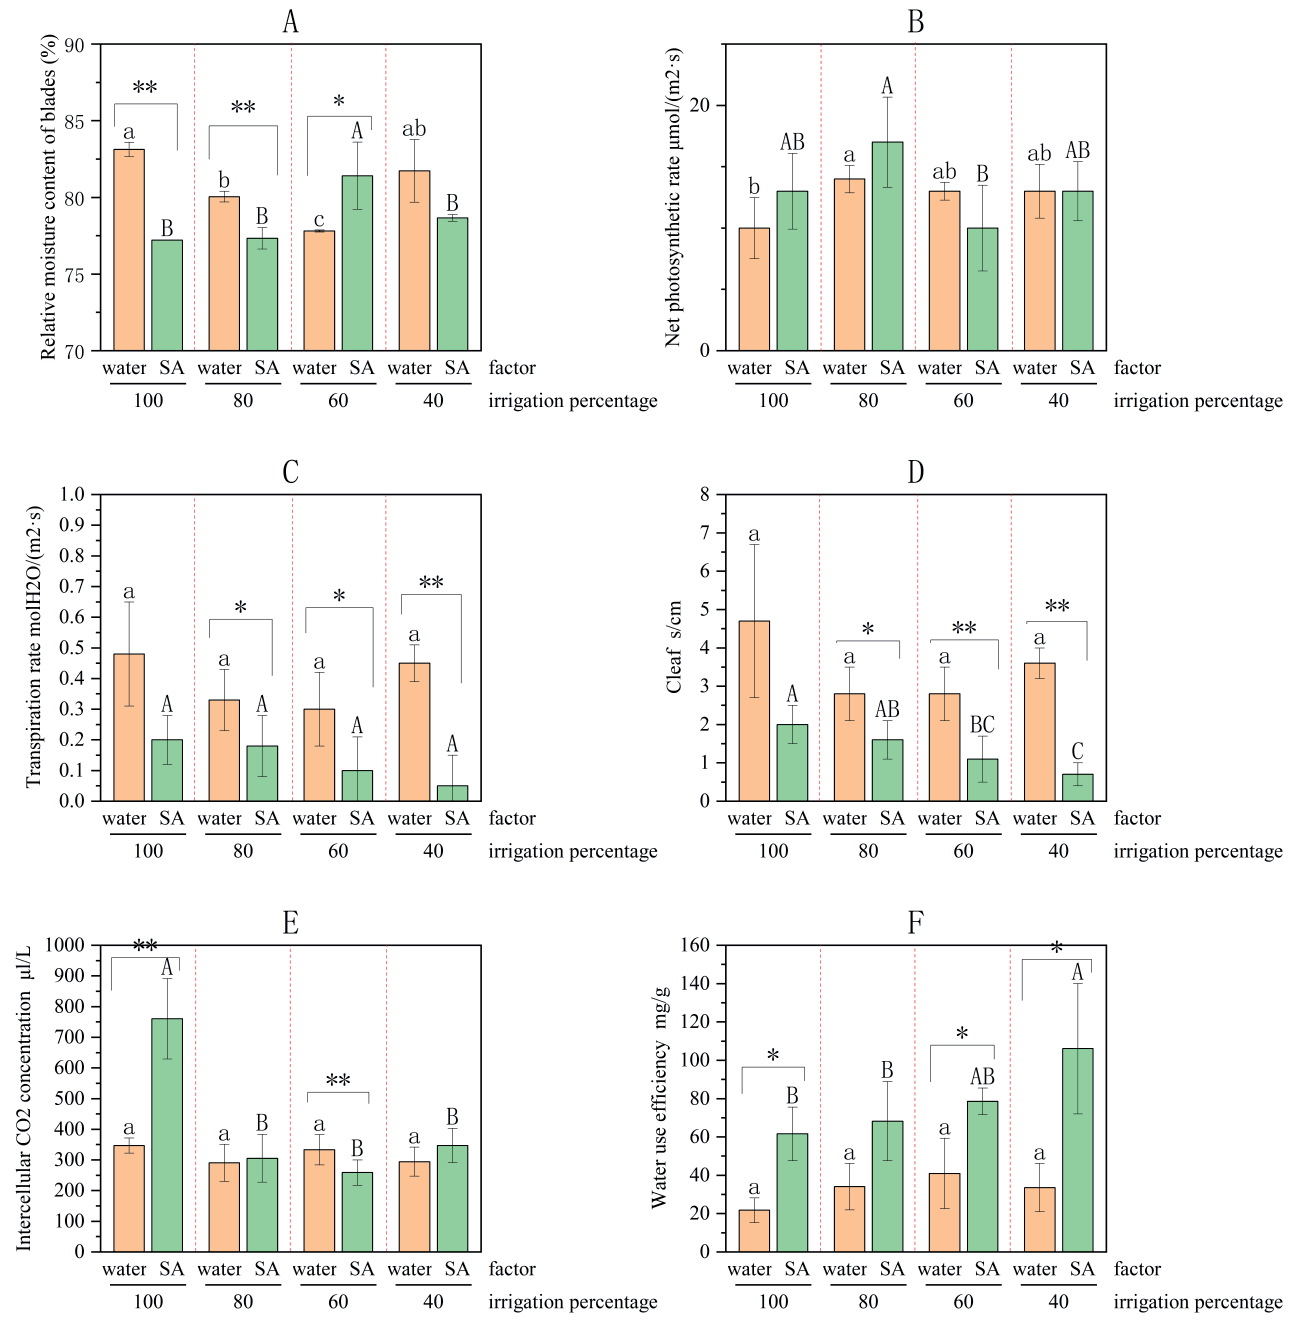
With the decrease in irrigation amount, the deficit level of sunflowers changed from 80% to 40%, and the relative water content of the leaves of sunflowers exhibited a decreasing trend (Fig. 1a). As the deficit degree intensified, the water content of sunflowers' leaves decreased by 7.9 percentage points from 83.1% after irrigation. With the decrease in irrigation amount after spraying SA, the relative water content of the sunflowers' leaves demonstrated a peak-shaped change, first decreasing and then increasing. The inhibitory effect of SA differed significantly under the normal and 80% irrigation (P < 0.01). The improvement effect of SA peaked at 60% irrigation, with a 3.6% increase compared to water treatment. The deficit 40% treatment resulted in a 3.2% increase compared to water treatment, with a statistically significant difference (P < 0.05). As a result, the sunflowers are believed to exhibit severe drought stress in response to irrigation restrictions. Spraying SA can effectively increase the water content in sunflowers' leaves when the deficit reaches 60% and 40%. These results demonstrate that SA effectively reduced leaf moisture content in sunflowers under normal and 80% irrigation and significantly increased it under 40% deficit irrigation, with 60% deficit irrigation being the turning point for regulation.
The photosynthetic indicators of the sunflowers performed differently under different levels of deficit irrigation (Fig. 1b). Deficit irrigation slightly increased the Pn of sunflowers' leaves, while spraying SA exhibited a relatively minor effect on the Pn of sunflowers (Fig. 1b). There was no significant difference in the Pn of sunflowers between normal irrigation and 40% deficit irrigation and between the irrigation water levels and the SA treatment group, indicating that SA has limited regulatory effects on the photosynthesis of sunflowers under deficit irrigation.
The Tr of sunflowers exhibited a trend of first decreasing and then increasing as the irrigation deficit intensified (Fig. 1c). Under mild to severe deficit irrigation conditions, the Tr of sunflowers was 68.4%, 63.2%, and 94.7% compared to the control. However, the differences were not significant. After spraying SA, Tr decreased to 42.1% of the original level under normal irrigation and decreased significantly under mild, moderate, and severe deficit irrigation, with transpiration rates decreasing from 25% to 87.5%. This implies that SA can effectively reduce the transpiration of sunflowers, thereby reducing water loss from the leaves.
The Cleaf of sunflower leaves decreased slightly under deficit irrigation conditions (Fig. 1d). After spraying SA, Cleaf decreased, and the decrease became more severe with an increasing degree of irrigation deficit. The Cleaf of sunflower leaves treated with 60%– 40% deficit irrigation decreased significantly. As the degree of deficiency changed from mild to severe, the Cleaf values of the SA treatment exhibited significant, extremely significant, and extremely significant decreases, respectively, compared to those without SA. These results indicate that SA can regulate the closure of sunflower stomata, and the more severe the deficiency, the stronger the regulatory effect.
The CO2in of sunflowers remained relatively stable under different deficit irrigation treatments (Fig. 1e). Comparing the data between spraying water and the SA treatment under the same deficit irrigation conditions, there was a significant difference between the two treatments at a deficit degree of 60% and no deficit, indicating that spraying SA on sunflowers under normal irrigation is not conducive to the utilization of intercellular CO2. However, when the deficit degree reaches 60%, SA can effectively promote the consumption of intercellular CO2 and improve photosynthesis in sunflowers.
The We of sunflowers increased slightly as the irrigation deficit intensified (Fig. 1f). However, the difference was not significant. After SA treatment, this upward trend intensified, and SA significantly improved the We of sunflowers under 40% deficit irrigation. Under the same deficit irrigation treatment conditions, spraying SA at 100%, 60%, and 40% significantly improved the We compared with water spraying, indicating that SA is beneficial for improving the We of sunflowers under normal irrigation, moderate drought, and severe drought conditions.
Fig. 1.
The effect of SA on the relative moisture content and photosynthetic indicators of sunflower leaves under different levels of deficit irrigation. (Note: The * represents the degree of significant difference based on the paired sample t-test (* P < 0.05; ** P < 0.01). The letters within the same series indicate significant differences between the different treatments (Duncan, P < 0.05). The lowercase letters represent significant differences between treatments within the spray group, while the uppercase letters represent significant differences between treatments in the spray SA group. The same is represented below. (A) Relative moisture content of blades, (B) net photosynthetic rate (Pn), (C) transpiration rate (Tr), (D) stomatal conductance (Cleaf), (E) intercellular CO2 concentration (CO2in), and (F) We.)
Firstly, as an endogenous plant hormone, SA plays a beneficial role when plants are under stress. Extensive research has shown that exogenous SA application improves stress adaptability of various crops, including wheat [4, 13, 19, 21, 26], soybean [6, 14, 20], pearl millet [18] and coffee beans [27], which aligns with the findings of the present study. Mechanistically, SA has been shown to regulate key physiological processes such as water use efficiency and photosynthetic performance. In this investigation, the SA application under drought conditions led to reduced transpiration rates and stomatal conductance in sunflower plants while promoting more efficient intercellular CO₂ utilization. These observations are consistent with previous reports demonstrating that SA enhances drought resistance in wheat through activation of stress-responsive genes, modulation of stomatal aperture, and increased chlorophyll content, ultimately leading to improved dry matter accumulation and yield [13, 19, 21]. Some researchers suggested giving a 25% deficit as an alternative to full irrigation of soybeans in the Mediterranean basin during water-scarce seasons, and SA can also play an important regulatory role [6].. However, a key methodological difference warrants attention. While previous studies on wheat and soybean employed relatively high SA concentrations (0.5 mM or 100 mg/L), the present study utilized a substantially lower concentration (20 mg/L). This discrepancy in application rates may lead to varying physiological responses across species, suggesting the need for further investigation to establish optimal SA dosages for different crops under drought stress conditions.
Secondly, in the context of global water scarcity, multi-model analyses confirm that climate change is intensifying the uneven distribution of water resources, with recent estimates suggesting that nearly 4 billion people experience at least one month of water shortage annually [28], of which irrigation agriculture remains a primary contributor. Given these challenges, SA emerges as a promising plant growth regulator, capable of enhancing drought adaptation. Moreover, the IPCC report has highlighted that global warming will have profound impacts on water security, with water scarcity projected to intensify by 2050 [29]. Therefore, the application of SA not only enhances the stress tolerance of crops but also partially alleviates water scarcity caused by climate change.
In conclusion, SA demonstrates species-dependent modulation but offers new solutions to global water scarcity by enhancing plant water-use efficiency and photosynthetic capacity.
Effects of SA on the Expression of Sunflower Proteome Under Deficit Irrigation
Effects of SA on the Protein Abundance of Sunflowers Under Deficit Irrigation
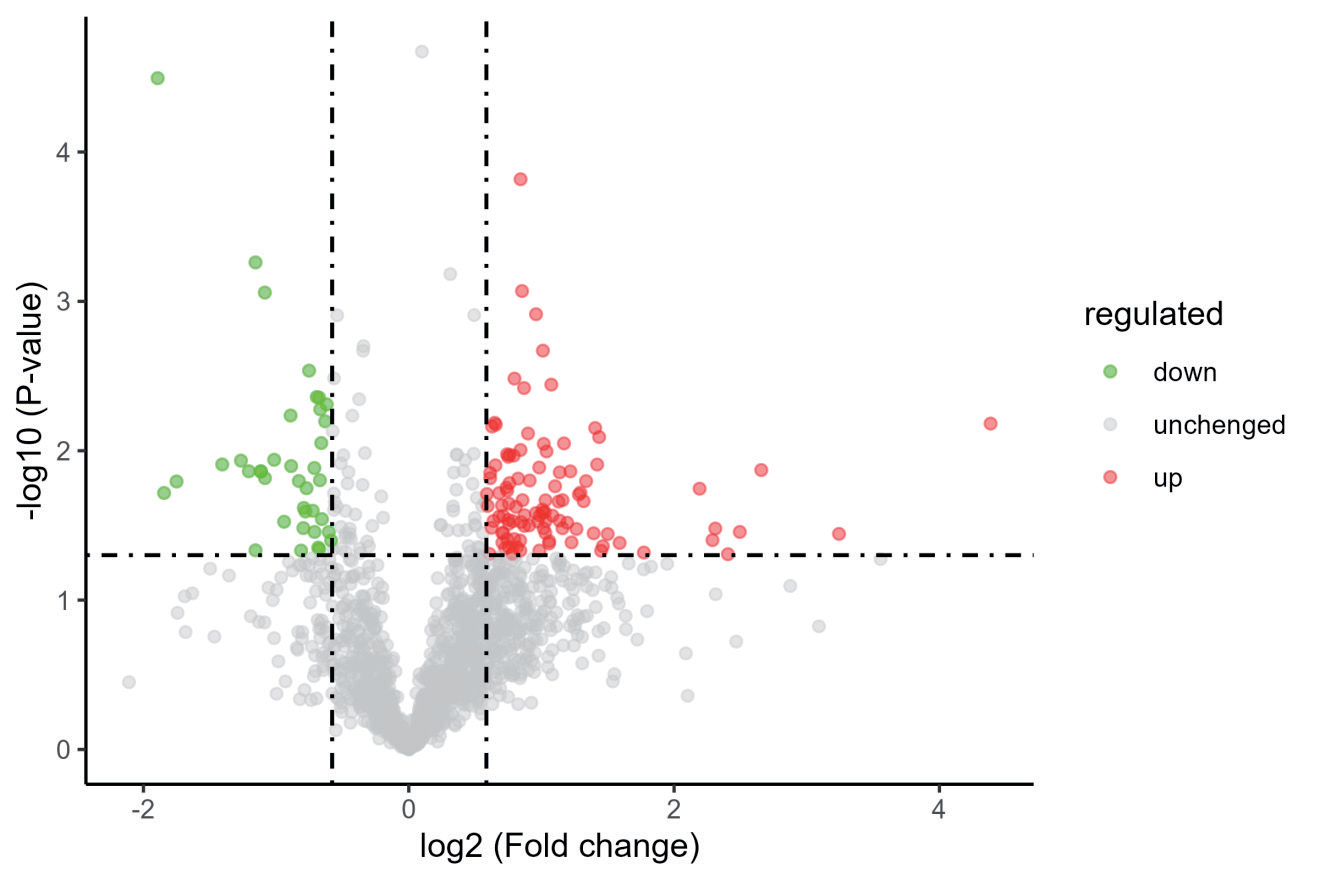
The Volcano Plot of differentially expressed proteins (Fig. 2) revealed that SA exhibited a certain regulatory effect on the protein abundance sample of deficit irrigated sunflowers compared with the control. A total of 1683 differentially expressed proteins were detected, of which 1541 were not significantly different, and 142 were significantly different. The reliability of the screening of differentially expressed proteins was similar.
Screening of Differentially Expressed Proteins between Sunflower SA Treatment and Control Under Deficit Irrigation
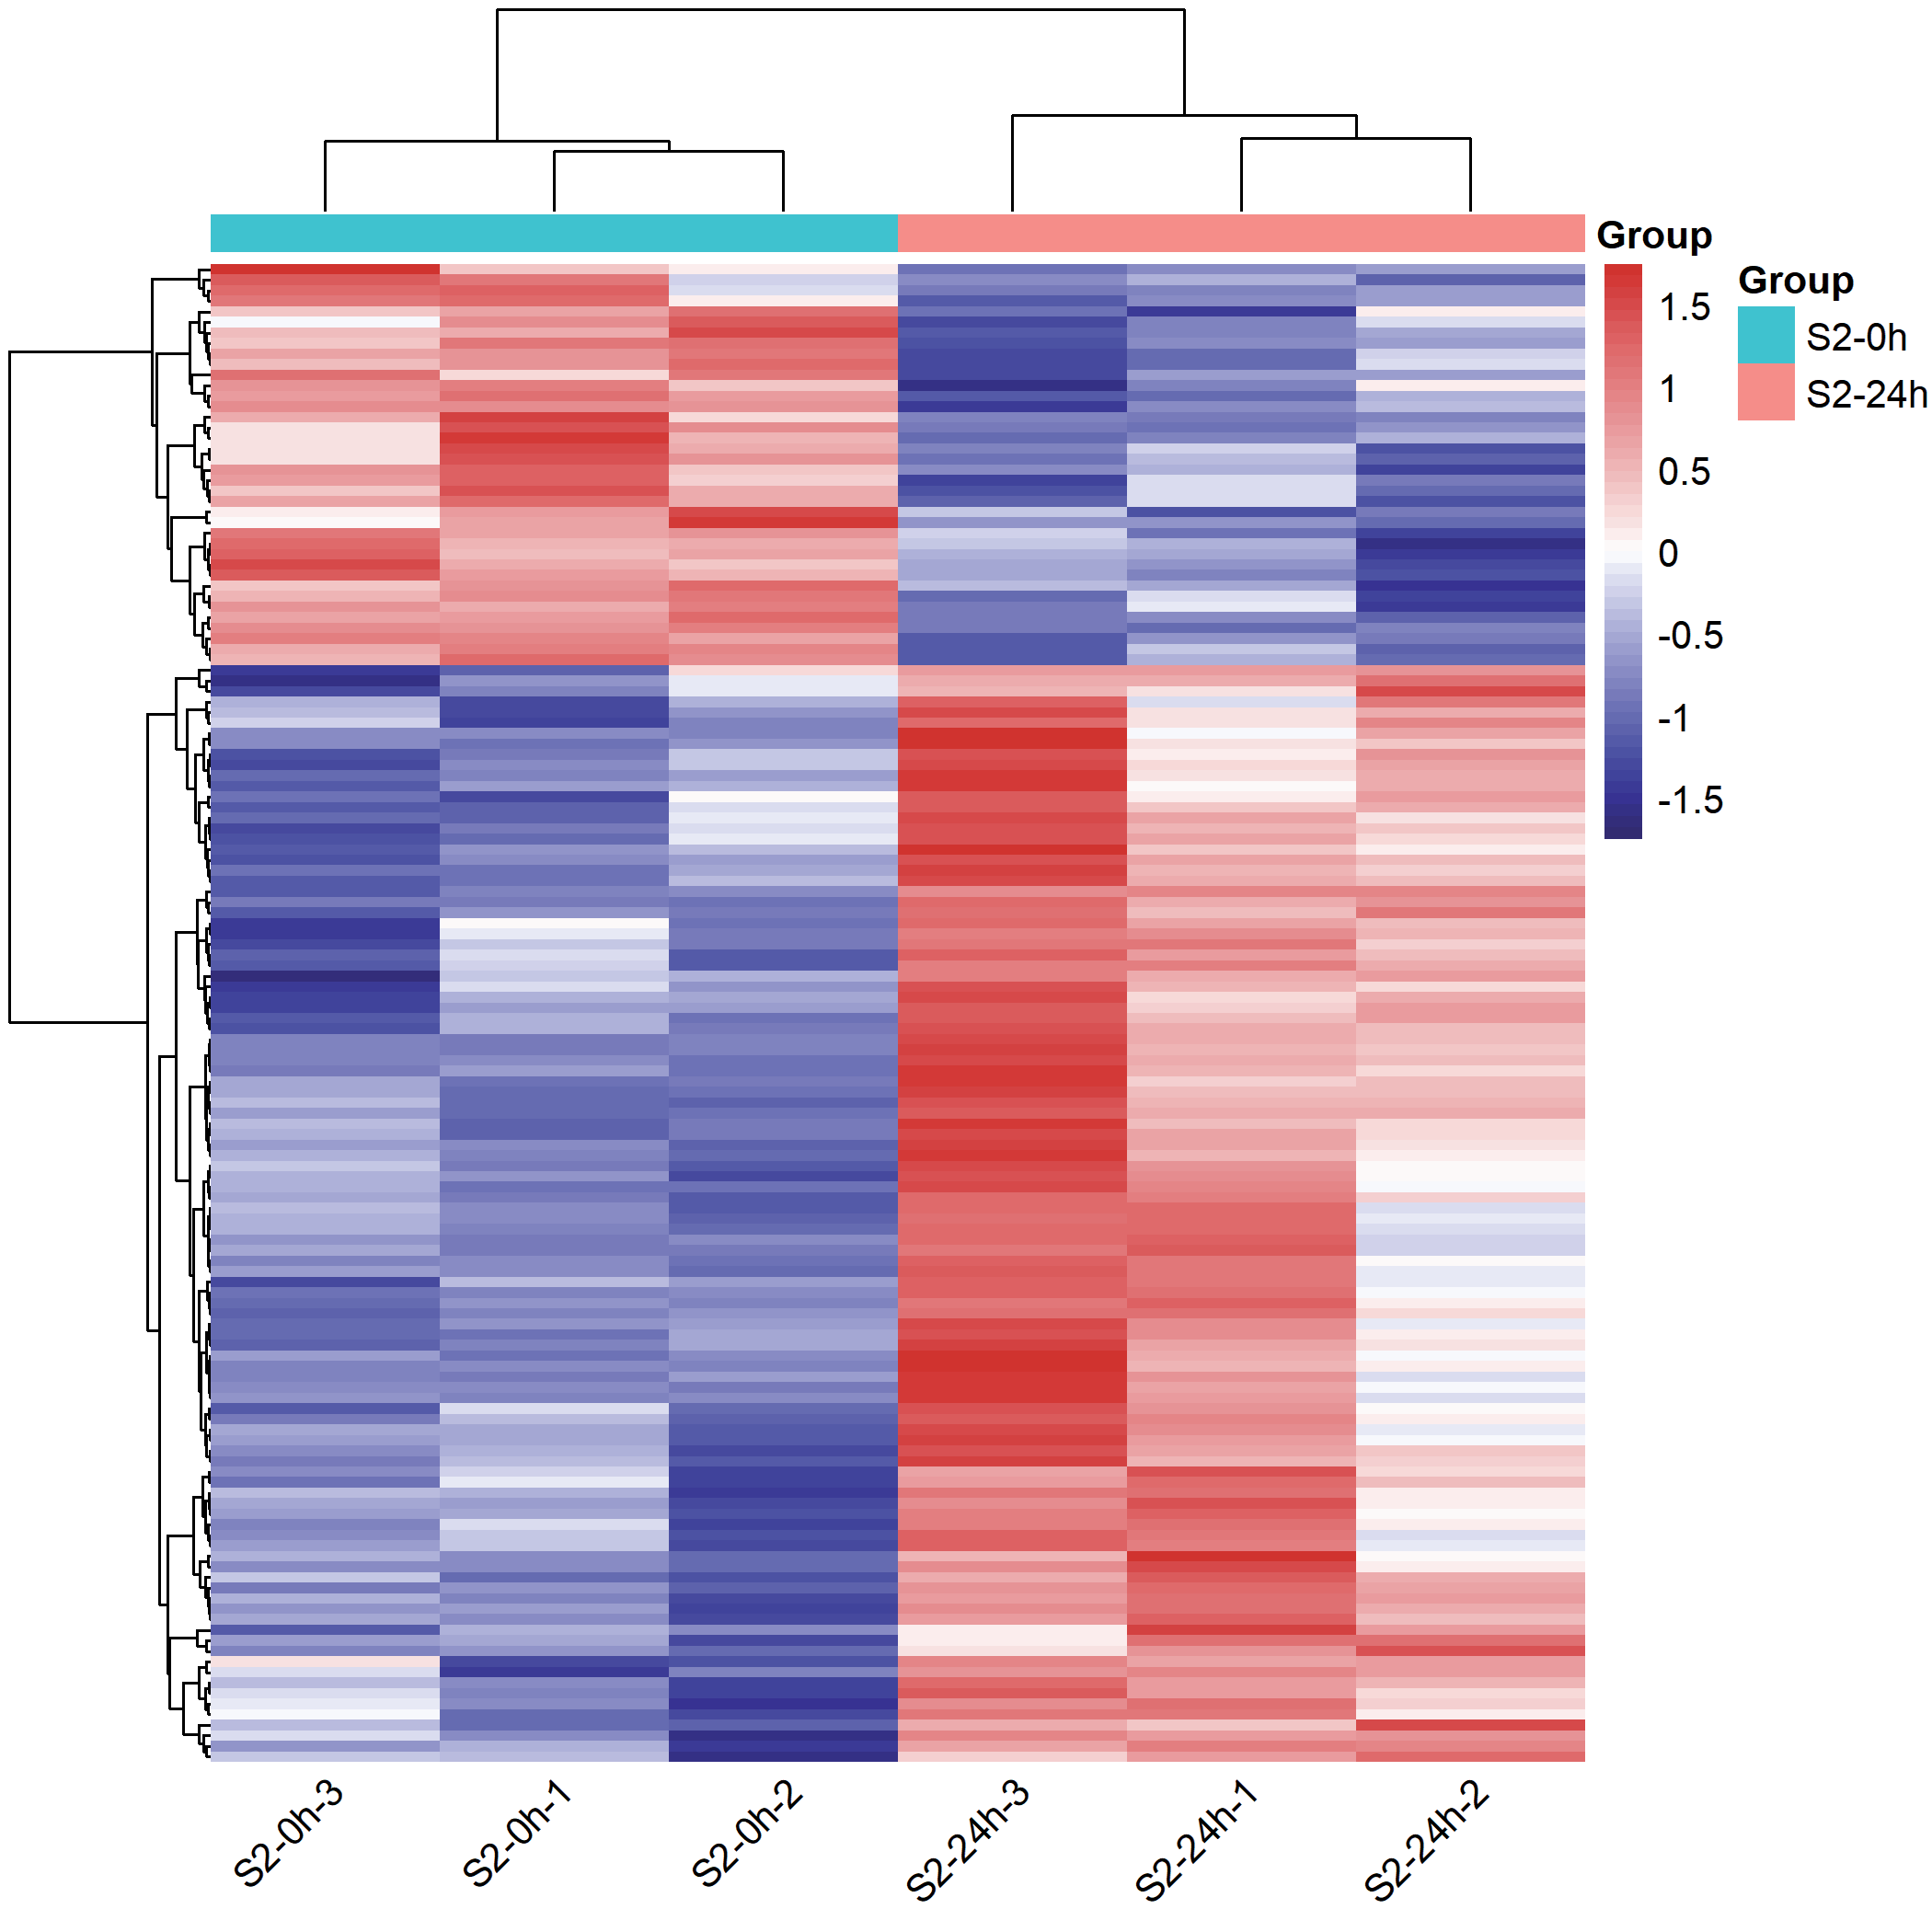
The clustering heatmap (Fig. 3) revealed that after SA treatment, the differential protein clustering analysis (Cluster Analysis) of drought sunflowers indicates that SA has a significant regulatory effect on the proteomics of sunflowers under deficit irrigation conditions. After SA treatment, there were 142 proteins with significant differences in drought sunflowers, including 104 upregulated and 38 downregulated proteins.
SA significantly up-regulated 104 proteins, of which 10 proteins’ activity was upregulated to more than three times, which were involved in “translation, ribosome structure, and biogenesis”, “carbohydrate transport and metabolism”, “signal transduction mechanism”, and “chloroplast thylakoid membrane synthesis”. The abundance of these four types of proteins was upregulated by 6.31, 4.89, 4.57, and 3.01 times, respectively. SA can increase protein abundance in response to a water deficit in sunflowers, serving as a signaling molecule that regulates RNA translation and processing, photosynthesis, and carbohydrate transport.
SA significantly downregulated 38 proteins, among which proteins related to "RNA processing and modification" were downregulated by up to 0.278 times, proteins related to "post-translational modification, protein turnover, and chaperones" were downregulated by up to 0.297 times, and proteins related to "carbohydrate transport and metabolism" were downregulated by up to 0.416 times. This indicates that RNA methylation and reverse transcription-related proteins are inhibited by SA, while the concentrations of carbohydrate transport metabolism-related proteins and lactose glutathione lyase were decreased. In deficit irrigated sunflowers, proteins related to RNA translation and processing and carbohydrate transport, and metabolism are the main targets of SA regulation.
COG Annotation Analysis of Differentially Expressed Proteins in Sunflowers Under Deficit Irrigation Under SA Treatment
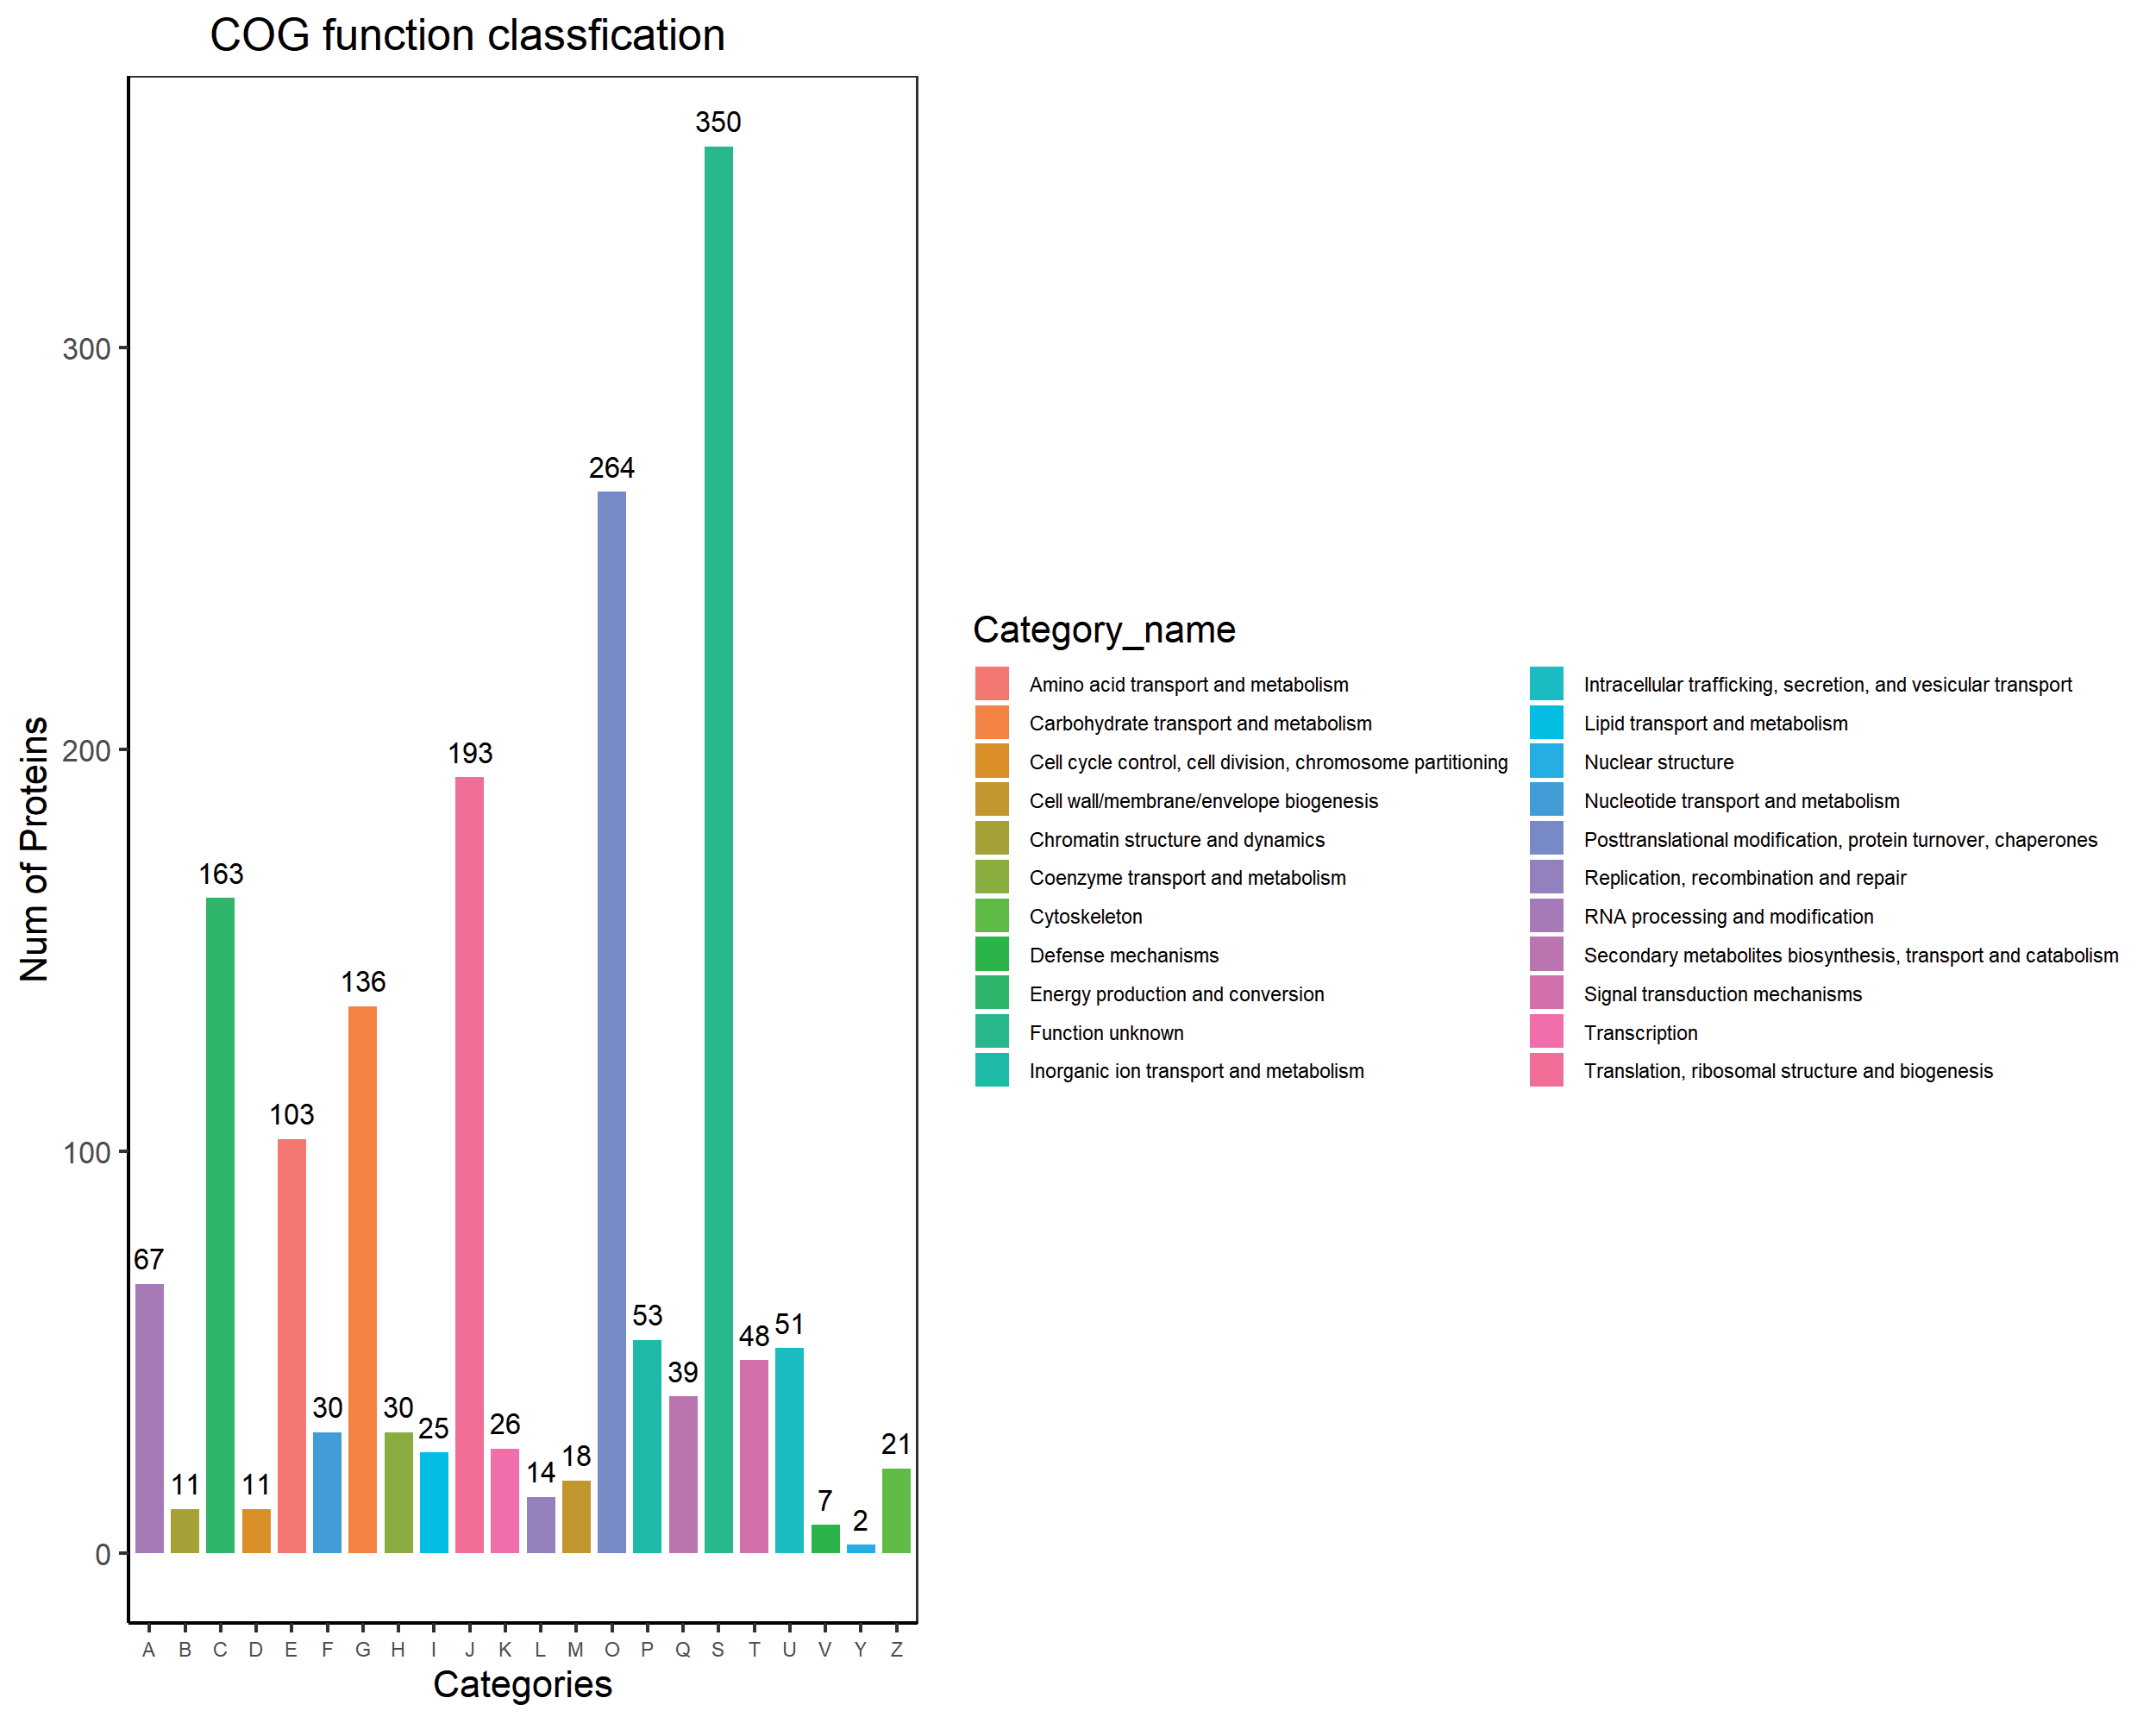
The annotation diagram of the differentially expressed protein COG in deficit irrigated sunflowers by SA is depicted in Fig. 4. The COG annotation revealed that there were 22 types of categories among the 1662 annotated protein functions, of which more than half of the protein functions were concentrated in the following six categories: post-translational modification and protein turnover and chaperones, translation and ribosomal structure and biogenesis, energy production and conversion, carbohydrate transport and metabolism, amino acid transport and metabolism, and RNA processing and modification. Additionally, the functions of 21.1% proteins were unknown. This indicates that SA is related to RNA translation and modification in sunflowers under deficit irrigation, which can accelerate photosynthesis and phosphorylation, release ATP and water, promote the synthesis of phenylpropanoid secondary metabolites, and regulate plant adaptability to the environment. It is speculated that SA improves the expression of genetic information in the body through phenylpropane metabolites, regulates photosynthesis, activates energy in the body, and releases water, thereby improving the drought resistance of sunflowers.
Fig. 2.
Volcano of differentially expressed proteins of Sunflower between SA treatments and the control under deficit irrigation. (Note: Each point in the volcano plot represents a protein, and the horizontal axis represents the fold change of each substance compared in the group (taking the logarithm with a base of 2). The vertical axis represents the P-value of the student's t-test (taking the logarithm with a base of 10). The size of the scatter represents the VIP value of the OPLS-DA model, and the larger the scatter, the greater the VIP value, indicating that the differentially expressed proteins selected are more reliable. The green dots in the figure represent down-regulated differentially expressed proteins, the red dots represent up-regulated differentially expressed proteins, and the black dots represent detected proteins with insignificant differences.)
Firstly, the molecular mechanisms of SA-mediated proteomic regulation under drought stress. The proteomic profiling in this study elucidates that SA orchestrates a sophisticated regulatory network in drought-stressed sunflowers. The pronounced upregulation of ribosomal proteins (6.31-fold) and chloroplast thylakoid membrane components (3.01-fold) suggests SA's dual role in maintaining protein synthesis fidelity and photosynthetic apparatus integrity under water deficit. This observation aligns with but extends previous findings in wheat by revealing sunflower-specific thylakoid membrane stabilization mechanisms [20, 30, 31].
Secondly, metabolic pathway cross-talk and stress adaptation. Notably, the coordinated regulation of carbohydrate transport proteins (4.89-fold upregulation) with concomitant suppression of RNA methylation enzymes (0.278-fold downregulation) implies SA's strategic rewiring of carbon allocation in sunflower. The results of this study share certain differences with those of previous studies on other plants. In the studies on soybean and cowpea, the regulatory functions of SA are primarily focused on carbohydrate metabolism, ATP synthesis, and plant signaling pathways [20, 30, 31]. This suggests that while the mechanisms of SA action in response to drought stress may be somewhat conserved across different plants, the specific pathways and targets regulated by SA may vary depending on the plant species. In studies on wheat and sorghum, drought stress-induced differentially expressed proteins are primarily involved in carbohydrate and energy metabolism, antioxidant defense, and transcriptional regulation. These processes collectively contribute to the plants' effective self-repair capabilities [12, 27, 32]. Similar to the findings in this study, sunflowers under SA regulation also exhibit significant responses in carbohydrate and energy metabolism. However, the role of SA in sunflowers extends further to the biosynthesis of phenylpropanoid secondary metabolites, which may represent a unique mechanism for sunflowers to adapt to drought stress.
Moreover, studies on the regulatory pathways of SA have demonstrated that SA can increase the relative water content, chlorophyll content, and water use efficiency in wheat leaves. The mechanism may involve enhancing seedling vigor by increasing the levels of potassium (K⁺), calcium (Ca²⁺), and magnesium (Mg²⁺) in the roots, thereby indirectly improving water use efficiency [26, 32]. This mechanism may also exist in sunflowers, but the current study focuses more on the regulation of protein metabolism and secondary metabolism by SA, providing a new perspective for understanding the diverse roles of SA in different plants.
Fig. 3.
Heatmap cluster analysis of differentially expressed proteins of Sunflower between SA treatments and the control under deficit irrigation.
In summary, this study has elucidated the role of SA in the drought response of sunflowers, particularly its regulation of protein metabolism, photosynthesis, and secondary metabolism. These findings corroborate the results of previous studies on other plants and also highlight the diversity and complexity of SA's functions across different plant species. Future research can further explore the conservation and specificity of the SA signaling pathway in various plants, as well as its synergistic mechanisms with other plant hormones, to provide a more comprehensive theoretical basis for enhancing plant drought resistance.
Subcellular Localization of Differentially Expressed Proteins in Sunflowers Under Deficit Irrigation Under SA Treatment
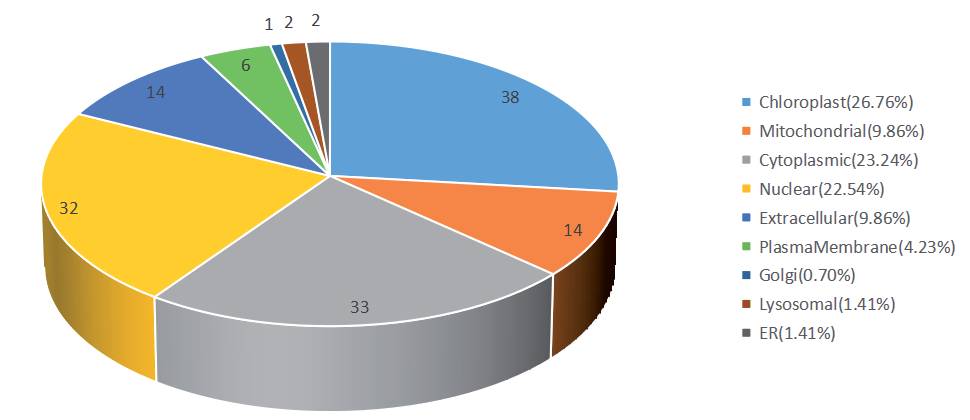
The subcellular localization map of differential proteins in sunflowers under SA-regulated deficit irrigation conditions (Fig. 5) demonstrates that the subcellular localization from high to low is as follows: chloroplasts, cytoplasm, nucleus, mitochondria, extracellular space, and a small portion is distributed in the cytoplasmic membrane, lysosomes, endoplasmic reticulum, and Golgi apparatus. Among them, proteins distributed in chloroplasts accounted for 26.76% of the differential protein types, whereas proteins distributed in the cytoplasm and nucleus accounted for 23.24% and 22.54%, respectively. This indicates that SA mainly regulates chloroplast photosynthesis and processes occurring in the cytoplasm and nucleus of the sunflower leaf cells.
This distribution pattern suggests that the mechanism by which SA responds to water stress may involve multiple mechanisms working in concert, including photosynthesis, intracellular metabolic activities, gene expression, and possibly energy metabolism and signal transduction. The differential proteins localized in chloroplasts indicate a critical role of SA in the process of carbon assimilation, enhancing CO2 utilization efficiency through regulating protein activity, as has been demonstrated in various plants such as popcorn, Pandanus amaryllifolius, and faba bean [33-35]. The enrichment of differential proteins in the cytoplasm/ nucleus might be associated with ROS signaling, resistance signal transduction, and transcriptional regulatory networks. Sun also demonstrated that dehydration-responsive element binding proteins (DREB) are localized in the nucleus of plants such as Allium cepa and faba bean, adding more scientific evidence to this notion [34-37]. Notably, the distribution of mitochondrial differential proteins implies that SA could enhance drought resistance by modulating energy metabolic balance, echoing previous findings in popcorn maize and sunflower [33, 35]. These discoveries provide new molecular evidence for unraveling the mechanisms of plant stress responses mediated by SA.
Fig. 4.
COG function of differentially expressed proteins of Sunflower between SA treatments and the control under deficit irrigation.
KEGG Metabolic Pathway of Differentially Expressed Proteins in Sunflowers Under Deficit Irrigation Under SA Treatment
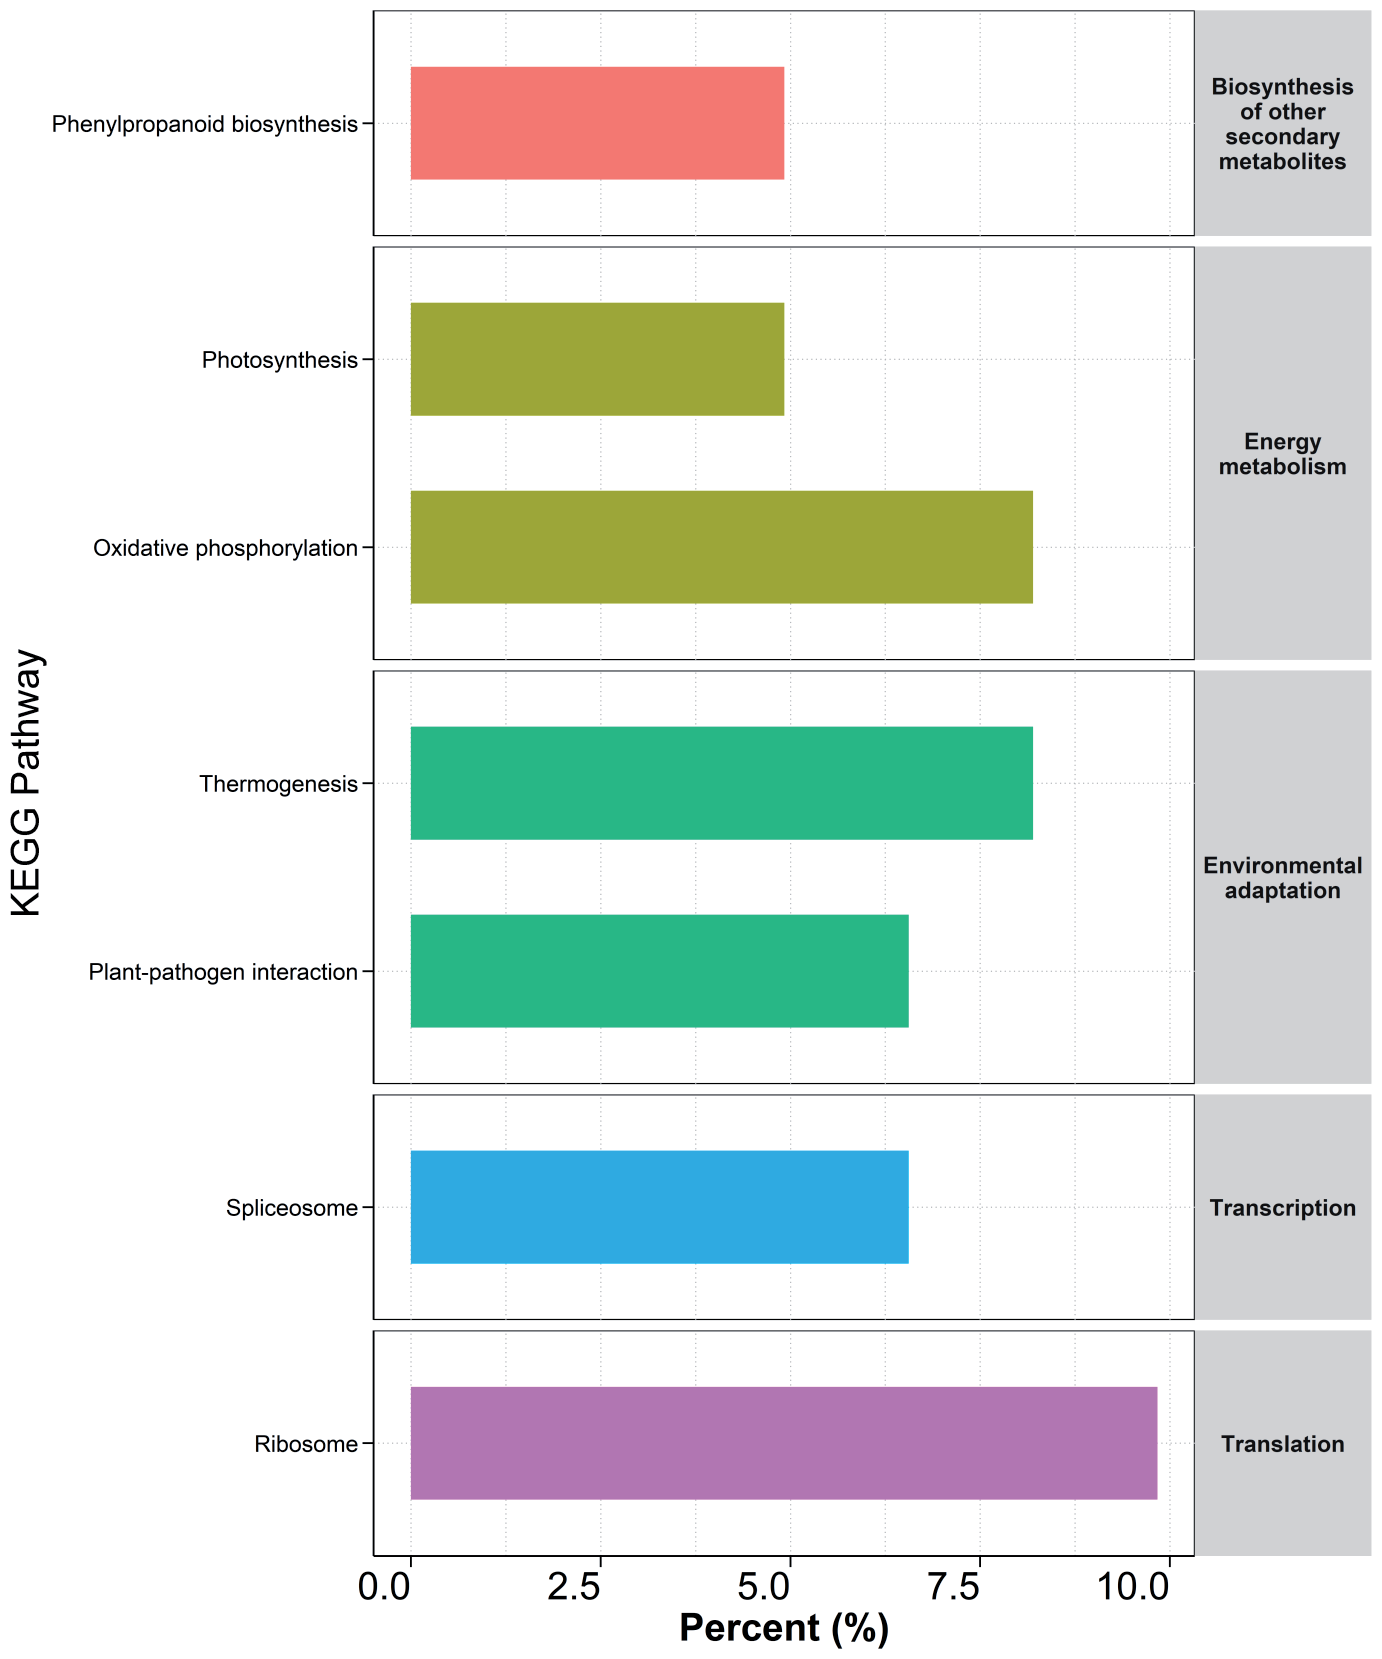
Differentially expressed proteins were mapped using the KEGG metabolic pathway (Fig. 6). KEGG pathway significance enrichment analysis revealed that the differentially expressed proteins treated with SA participated in spliceosome, ribosome, photosynthesis, oxidative phosphorylation, thermogenesis, plant-pathogen interaction, and phenylpropanoid biosynthesis processes. These metabolites belong to the following pathways: translation, transcription, energy metabolism, environmental adaptability, and secondary metabolites biosynthesis. Under water deficit conditions, sunflowers are affected by SA, thereby improving the expression of genetic information, accelerating photosynthesis, consuming organic matter, releasing internal heat, and stimulating secondary metabolic pathways. It is hypothesized that with water deficiency, SA acts as a signaling substance that accelerates a series of metabolic pathways in sunflowers, regulating the balance of substances and energy, and also stimulating phenylpropanoid biosynthesis metabolism to assist in enhancing stress resistance.
Under water-deficient conditions, SA may enhance drought resistance in sunflowers through the following mechanisms: regulating ribosomal protein expression levels to maintain translational efficiency, activating the turnover and repair of specific proteins in chloroplast reaction centers, and enhancing lignin biosynthesis through key enzymes such as phenylalanine ammonia-lyase (PAL), thereby reinforcing the mechanical strength of cell walls. It is noteworthy that SA-induced metabolic reprogramming exhibits systemic regulatory characteristics, encompassing both organelle-specific functional adjustments (e.g., chloroplast photosystem repair) and multi-level coordinated mechanisms involving transmembrane signaling and epigenetic regulation (e.g., histone modifications). This multi-target regulatory mode shows conservation in Brassicaceae [36, 38], Poaceae [19, 39], and Fabaceae plants[31, 35], suggesting the evolutionary advantage of SA as a systemic signaling molecule in plant stress adaptation.
In summary, the study preliminarily reveals partial mechanisms through which SA regulates sunflower responses to water deficit stress. Further investigations, including identification of target genes and functional validation, are required to provide a theoretical foundation for improving agricultural irrigation efficiency and developing water-saving farming practices.
Conclusions
(1) SA improved the water content of sunflowers under 40% water deficit conditions, and remained stable under a 60% deficit condition. The inhibitory effect of SA on transpiration rate and stomatal conductance gradually increased with the aggravation of the water deficit. Therefore, SA effectively improved We within a deficit range of 40%–60%, and promoted the consumption of intercellular CO2 under a 60% water deficit.
(2) In sunflowers under 60% water deficit conditions, 142 out of the 1,683 differential proteins showed significant changes. SA not only upregulated 104 proteins involved in key physiological processes such as RNA translation, photosynthesis, and carbohydrate transport but also downregulated 38 proteins involved in processes such as RNA methylation and reverse transcription. Moreover, the COG annotation revealed that SA stimulated various functional proteins in sunflowers and regulated translation and transcription processes, as well as the conversion of energy, carbohydrates, and amino acids.
(3) The subcellular localization of differentially expressed proteins is mainly distributed in the chloroplasts, cytoplasm, and nucleus, indicating the diversity of target sites for SA regulation.
(4) The KEGG pathway enrichment analysis revealed that SA enhances the translation and transcription of genes, strengthens photosynthesis, activates energy, and releases water, initiating phenylpropanoid secondary metabolite signaling in sunflowers.
In summary, SA was sprayed on sunflowers under water deficit conditions, targeting proteins in the chloroplasts, cytoplasm, and nucleus. By mobilizing the release of phenylpropanoid signaling substances in the body, it induces translation and transcription, promotes the utilization of CO2 by plant cells, increases energy supply in the body, increases the concentration of sugar substances in photosynthetic products, closes stomata, and reduces evaporation, thereby preserving the water content in the leaves and normal metabolism of cells, which is beneficial for plant growth and repair. This could be beneficial for sunflowers to repair the damage caused by the water deficit, helping to alleviate water limitations and, to some extent, improving agricultural We.

