

Introduction
Long-term continuous cropping and poor tillage practices easily lead to unfavorable changes in soil physicochemical properties and alter the composition and diversity of soil microbial communities, leading to a series of challenges commonly observed under continuous cropping systems, including soil acidification, salinization, and soil-borne diseases [1]. Soil-borne diseases are difficult to control, prone to recurrence, and highly detrimental, seriously affecting crop yield and quality. The formation of soil-borne diseases is closely associated with the imbalance of soil microbial communities, often characterized by a significant decline in beneficial bacteria and a corresponding increase in pathogenic bacteria [2]. Therefore, restructuring the soil microbial community and improving the soil microecological balance are crucial for controlling soil-borne diseases in continuous cropping systems. Long-term, uninterrupted cultivation has been shown to have adverse effects on soil health in multiple ways. It degrades soil physicochemical properties, disrupts enzyme activities involved in carbon, nitrogen, and phosphorus cycling, and leads to the buildup of autotoxins. These changes collectively contribute to a decline in soil microbial diversity and ecological function [3].
Soil microorganisms play a vital role in soil nutrient cycling, the occurrence and prevention of soil-borne diseases, and the growth and development of crops. They dominate the decomposition of soil organic matter, maintain soil fertility, and support soil health through a stable microbial community structure and rich microbial diversity. Thus, soil microorganisms are the most active component of the soil and serve as important indicators of the soil ecosystem. Numerous studies have concluded that the main cause of crop succession disorders is the alteration of soil microorganisms. Long-term continuous cropping reduces the population of beneficial microbial communities and increases the abundance of harmful microbial communities [4, 5]. Research has shown that bacterial diversity and the abundance of beneficial bacteria were significantly reduced in soils where tobacco was continuously grown for different durations [6]. Similarly, continuous cropping of konjac and potato altered the structure and diversity of soil bacterial communities [7, 8]. Moreover, continuous cropping often results in the enrichment of soil-borne plant pathogens such as Fusarium in the rhizosphere soil [5, 9].
At present, soil sterilization technology is the most common and effective method for preventing and controlling soil-borne diseases in agricultural production practices. This technology primarily achieves its effect by efficiently and rapidly eliminating fungi, bacteria, nematodes, and other harmful organisms in the soil [10]. Pre-planting soil fumigation is the most direct and effective method for controlling soil-borne fungal pathogens, nematodes, and weeds. Examples of commonly used soil fumigants include chlorpyrifos (CP), 1,3-dichloropropene (1,3- d), and products based on metam compounds (metam-sodium and metam-potassium) are widely used to control soil-borne diseases and improve strawberry crop yields. Solarization is a commonly used physical disinfection method, which raises the surface soil temperature above 50 °C to kill temperature-sensitive microorganisms. Lime nitrogen and dazomet are the two most commonly used chemical disinfectants. Both disinfect the soil through reactions with water, but the active substances produced differ: lime nitrogen generates cyanamide and dicyandiamide [11], while dazomet produces methyl isothiocyanate [12]. The duration of a disinfectant’s impact on non-target soil microorganisms can vary [13], necessitating further research to clarify these interactions. Understanding the effects of soil disinfectants on microbial abundance and diversity is critical, as microorganisms play vital roles in soil quality, nutrient cycling, plant growth, stress resistance, and environmental detoxification [14-17].
Strawberry is a perennial evergreen herbaceous plant with high nutritional and economic value. However, with the expansion of facility agriculture, the cultivation area of strawberries under controlled conditions has increased annually, leading to more severe succession disorders. This has promoted the breeding and spread of soil-borne diseases such as yellow wilt, blight, root rot, green blight, and nematode infestations [18], resulting in drastic declines in strawberry yield and quality, which severely restricts production and development. Current soil-borne disease control techniques for strawberries include the selection of superior varieties, crop rotation, biological control, chemical disinfection using dazomet and metam sodium, and physical disinfection using solarization or hot water. Despite the widespread use of soil disinfection, a significant gap remains in understanding the comparative long-term effects of diverse disinfection methods (physical, chemical, and biological) on both soil physicochemical properties and the intricate microbial community structure under standardized field conditions. This lack of comprehensive comparative data hinders informed decision-making for sustainable crop management. In this study, solarization, dazomet fumigation, lime nitrogen application, and biofumigation were selected for soil disinfection in strawberry greenhouses suffering from severe succession barriers. We assessed their effects on soil physicochemical properties, bacterial and fungal community diversity, and predicted microbial functions. The findings aim to provide new theoretical insights and practical guidance for mitigating continuous cropping obstacles and improving the sustainability of strawberry production systems.
Material and Methods
Experimental Site and Soil Sampling
Lime nitrogen was produced by Shizuishan Pengsheng Chemical Co., Ltd. with a purity ≥60%, and dazomet was produced by Nantong Shijiang Chemical Co., Ltd. with a purity ≥98%. The biological smothering agent (100 kg of Fertility Godfather and 400 g of soil conditioner) was produced by Beijing Jiabowen Biotechnology Co.
Experimental Design
The experiment was conducted from July 2024 to September 2024 in a monoculture greenhouse at the Zhijiang Base of the Hangzhou Institute of Agricultural Science (29°39′25″ N, 119°35′38″ E). Prior to the experiment, the shed had experienced more than four years of continuous strawberry cropping and exhibited severe succession barriers. These post-treatment samples were used for both soil physicochemical property analysis and macro-genomic (metagenomic) sequencing. The entire process, from treatment application to final sampling, was completed within the study period of July to September 2024. Before soil sterilization, soil samples were collected using the five-point method, mixed thoroughly, placed in sampling bags, and stored at -80°C for subsequent macro-genomic analysis. The pre-treatment samples were not considered as control (CK) samples, but rather as baseline references prior to treatment. The basic physicochemical properties of the test initial greenhouse soil were determined as follows: sandy loam texture, pH 8.20, conductivity 23.03 mS·cm⁻1, total organic carbon 0.48%, total nitrogen 0.41 g·kg⁻¹, available phosphorus 21.03 mg·kg⁻1, and available potassium 165.67 mg·kg⁻1.
The soil before disinfection served as the control (CK), with four treatments applied: solarization (SE), lime nitrogen (LN), dazomet (DA), and biofumigation (EM). Each treatment had three replicates, with each plot covering 50 m2 and separated by 1 m intervals. A total of 18 plots were established, covering approximately 1,333.33 m2, with protective rows arranged between them.
After removing the previous strawberry residues, the soil was fully tilled and mixed to a depth of approximately 20 cm. After repairing the old greenhouse film or replacing the new greenhouse film with a full seal, the soil is deeply turned over and leveled, irrigated to saturation until the surface of the ground sees bright water, covered with a film, and treated with cumulative high temperature (temperature of 35℃ or more) for at least 2 months. Lime nitrogen (10 kg per 667 m2 at 75% purity) and dazomet (10 kg per 667 m2 at 95% purity) were evenly applied to the test plots. The biofumigant, consisting of Fertility Godfather and soil conditioner at a weight ratio of 5:2, was evenly applied to the soil surface and thoroughly mixed into the soil using a rotary tiller. The soil was then irrigated to saturation and covered with a compression film to create anaerobic conditions. The external greenhouse film was also sealed to limit air exchange. After 15 days, the plastic film was removed to complete the biofumigation process. The 15-day sealing duration was selected based on the peak period of bioactive compound release during organic matter decomposition, as supported by prior studies. Subsequently, drip irrigation tubes were installed, and the plots were mulched with a new film of at least 0.8 mm thickness to ensure sealing. Irrigation through the drip system maintained soil moisture between 50% and 70%. “At the end of each disinfection period (e.g., 40 days for solarization), the plastic film was removed, and post-treatment soil samples were collected using the same five-point method as before. For fumigant-treated soils, samples were first aerated under a chemical fume hood to allow dissipation of residual gases. All samples were then stored at –80 °C for further metagenomic and physicochemical analyses.”
Metagenomics Determination
The specific sequencing platform used in our study was Illumina NovaSeq 6000. Fastp (http:github.com/ OpenGene/fastp) was used to trim adapter sequences at the 3' and 5' ends of reads. Reads with a quality cut length less than 50 bp, average quality score below 20, or containing N bases were removed to retain high-quality reads. Single-end reads were merged with paired-end reads [13]. Megahit (http://github.com/voutcn/megahit) was used to assemble the sequences, with a minimum contig length of ≥300 bp. The assembly was performed using MEGAHIT v1.2.9 with default k-mer sizes ranging from 21 to 141 in steps of 20 (i.e., 21, 41, 61, 81, 101, 121, 141). Contigs were subjected to ORF prediction using MetaGene version 2.0 (http: //metagene.cb.k.u-tokyo. ac.jp/), and gene sequences ≥100 bp were translated into amino acid sequences for sample gene prediction. We evaluated assembly metrics such as N50, total assembly size, and number of contigs ≥500 bp, using QUAST (Quality Assessment Tool for Genome Assemblies). Additionally, we used CheckM to assess completeness and contamination of metagenome-assembled genomes (MAGs), where applicable.
Clustering was performed with CD-HIT version 4.8.1 (http: //www.bioinfor⁃matics.org/cd-hit/) using default parameters (90% identity, 90% coverage) to establish a non-redundant gene set, selecting the longest gene in each cluster as the representative sequence [14]. SOAPaligner/soap2 version 2.21 (http: //soap.genomics. org.cn/) was used to align high-quality reads against the non-redundant gene sets (default 95% identity) to obtain gene abundance information [15].
Species taxonomic information was annotated using Diamond (version 0.8.35) (http: //www.diamondsearch. org/in⁃dex.php) with BLASTP alignment against the NCBI non-redundant (nr) protein database with an e-value threshold of 1e-5 [16]. Carbohydrate-active enzyme annotations were obtained using hmmscan (http: //hmmer.janelia.org/search/hmmscan) with the CAZy database (dbCAN HMMs v10 with an e-value threshold 1e-5. Annotation of ARGs resistance functions was conducted using DIAMOND BLASTP (e-value threshold 1e-5) against the Comprehensive Antibiotic Resistance Database (CARD, version [e.g., 3.2.3]
Determination of Physicochemical Properties
Soil salinity was measured using a conductivity meter (DDS-308A). Soil pH was measured with a pH meter (pHS-3C). Soil organic carbon (SOC) was directly determined using a TOC analyzer (multiN/C 2100S, Analytik Jena) after pretreatment to remove inorganic carbon. Soil total nitrogen was measured by the Kjeldahl method. Available phosphorus was determined by the sodium bicarbonate extraction method, and available potassium was measured using 1.0 M ammonium acetate (NH₄OAc) and subsequently measured using a flame photometer. All measurements were conducted at the same time as microbial sampling, after the completion of the soil disinfection treatments.
Data Analysis
Significant differences among treatments (Least Significant Difference, LSD, P<0.05) were analyzed using SPSS 12.0. Normality was assessed using the Shapiro–Wilk test, and homogeneity of variance was evaluated using Levene’s test. Species abundance at different taxonomic levels was assessed using QIIME 2 (version [e.g., 2021.4]), and microbial abundance maps and α-diversity boxplots were generated with Origin 2021. Pearson Correlation coefficients between samples were calculated using the Psych package in R 4.1.3. Microbial molecular ecological network thresholds were constructed based on Random Matrix Theory (RMT), available at http://ieg4.rccc.ou.edu/ mena/. Data visualization was conducted using Gephi 0.9.3. Functional prediction of soil microorganisms was conducted using Tax4Fun version 1.0, based on the KEGG database release 94.2. Visualization of predicted functional profiles was carried out using STAMP. The correlation between microbial communities and physicochemical factors was analyzed using a Mantel test via the ggcor package in R 4.1.3. RDA analysis was conducted using Canoco 5 software.
Results
Effects of Different Soil Sterilization Methods on Physicochemical Properties of Continuous Cropping Soil
As shown in Table 1, soil pH increased by 0.61%, 1.71%, and 0.49% in the SE, LN, and EM treatments, respectively, compared to the CK treatment, but decreased significantly by 1.59% (p<0.05) in the DA treatment. Soil EC increased significantly by 42.29% (p<0.05) in the DA treatment and by 7.82% in the LN treatment compared to CK, although the latter increase was not significant. In contrast, EC decreased by 22.28% and 7.82% in the SE and EM treatments, respectively.
Table 1.
Effects of different soil sterilization methods on physicochemical properties of continuous cropping soil.
Total soil nitrogen increased significantly by 43.90% (p<0.05), 4.88%, and 19.51% in the LN, EM, and DA treatments, respectively, compared to CK, but decreased by 2.44% in the SE treatment. Different treatments significantly decreased soil available phosphorus content, with reductions of 19.02%, 14.88%, 13.60%, and 19.16% (p<0.05) in the SE, LN, EM, and DA treatments, respectively. Soil available potassium content increased by 2.81%, 1.61%, and 3.62% in the LN, EM, and DA treatments, respectively, compared to CK, though the differences were not significant. In the SE treatment, the content of soil available potassium decreased by 4.63% compared to the control. Moreover, all treatments resulted in a significant reduction in soil organic carbon content, indicating a consistent decline in soil organic matter across different fertilization regimes. Soil effective phosphorus decreased significantly in the SE, LN, EM, and DA treatments by 6.25% (p<0.05), 20.83% (p<0.05), 18.75% (p<0.05), and 14.85%, respectively, compared to CK.
Effects of Different Disinfection Methods on Microbial Diversity
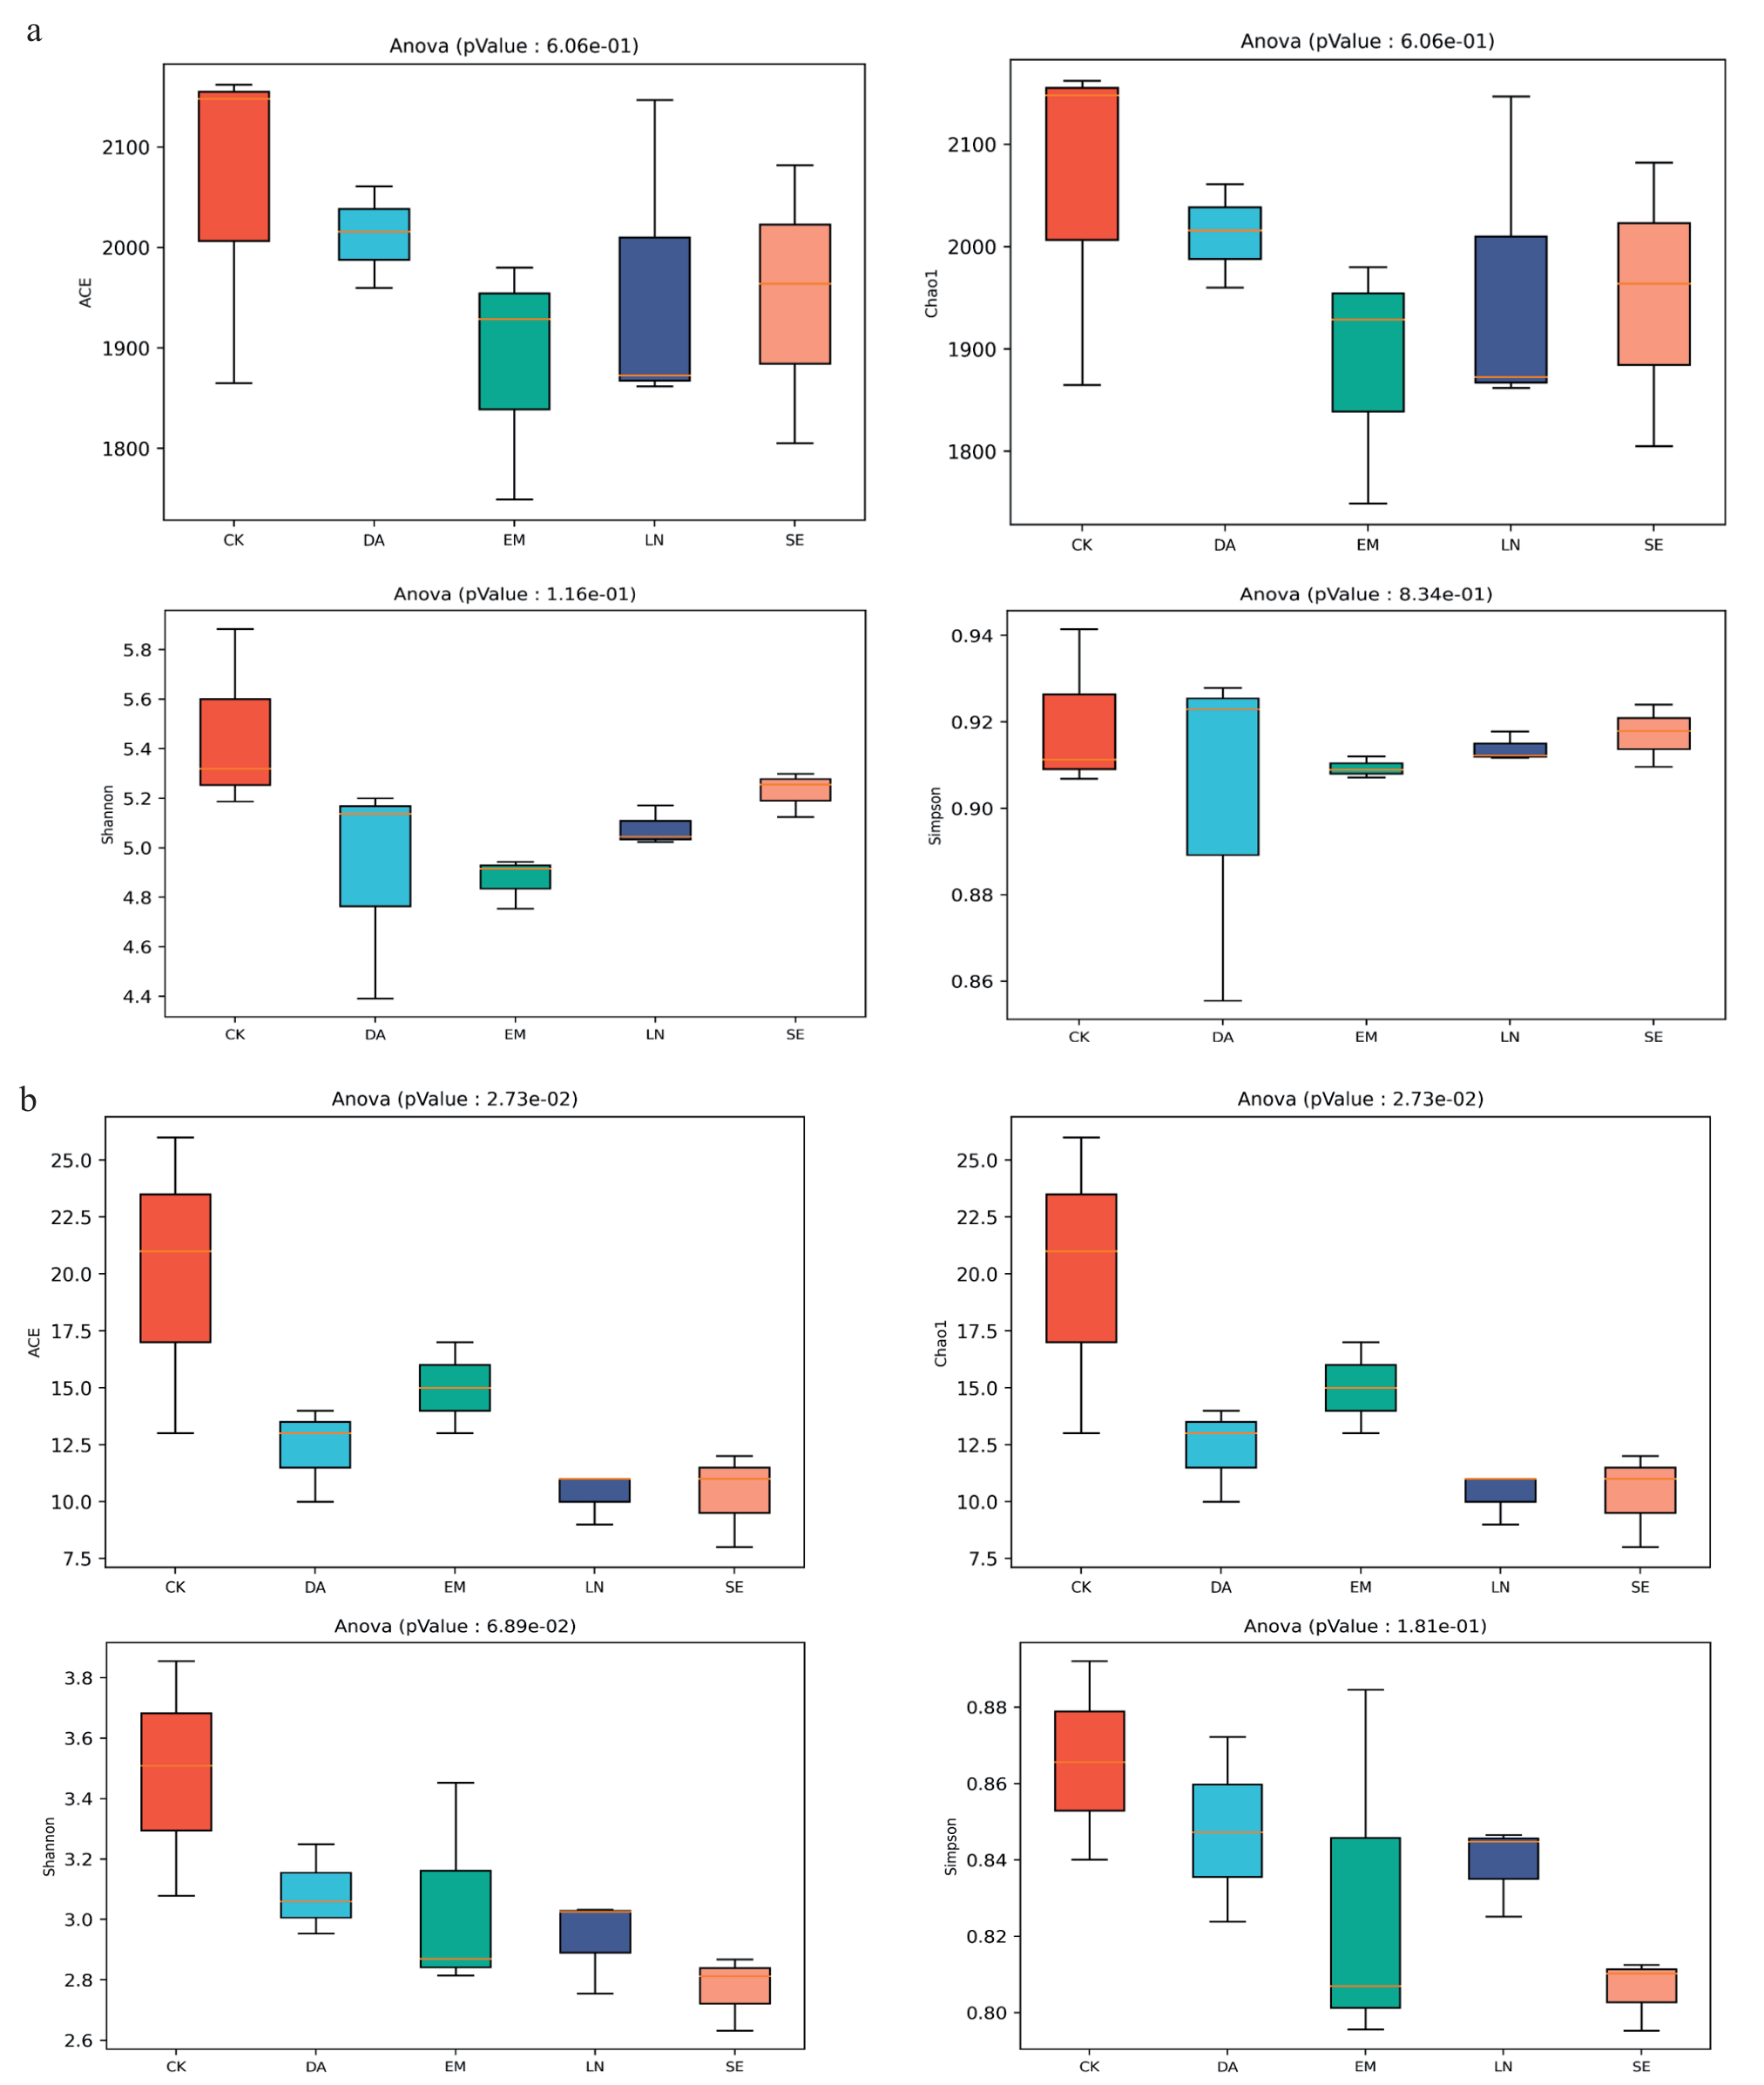
The Alpha diversity analysis of soil microbial communities after different disinfection treatments is shown in Fig. 1a. DA, EM, LN, and SE treatments all reduced the diversity and richness of bacterial communities to varying degrees. Among them, the ACE index, Chao index, Shannon index, and Simpson index were most significantly reduced in the EM treatment, with significant differences observed between groups. The EM treatment showed the most significant reduction in all four alpha diversity indices (ACE, Chao, Shannon, and Simpson) for bacterial communities compared to other treatments (p < 0.05). The ACE index, Chaol index, Shannon index, and Simpson index of fungal communities were significantly lower in the LN treatment compared to the other treatments, indicating that LN significantly reduced the richness of the strawberry continuous cropping fungal community.
These results suggest that different soil disinfection treatments had varying impacts on the microbial diversity of strawberry soil, with EM having a pronounced effect on bacterial diversity and LN showing a significant impact on fungal diversity (Fig. 1b).
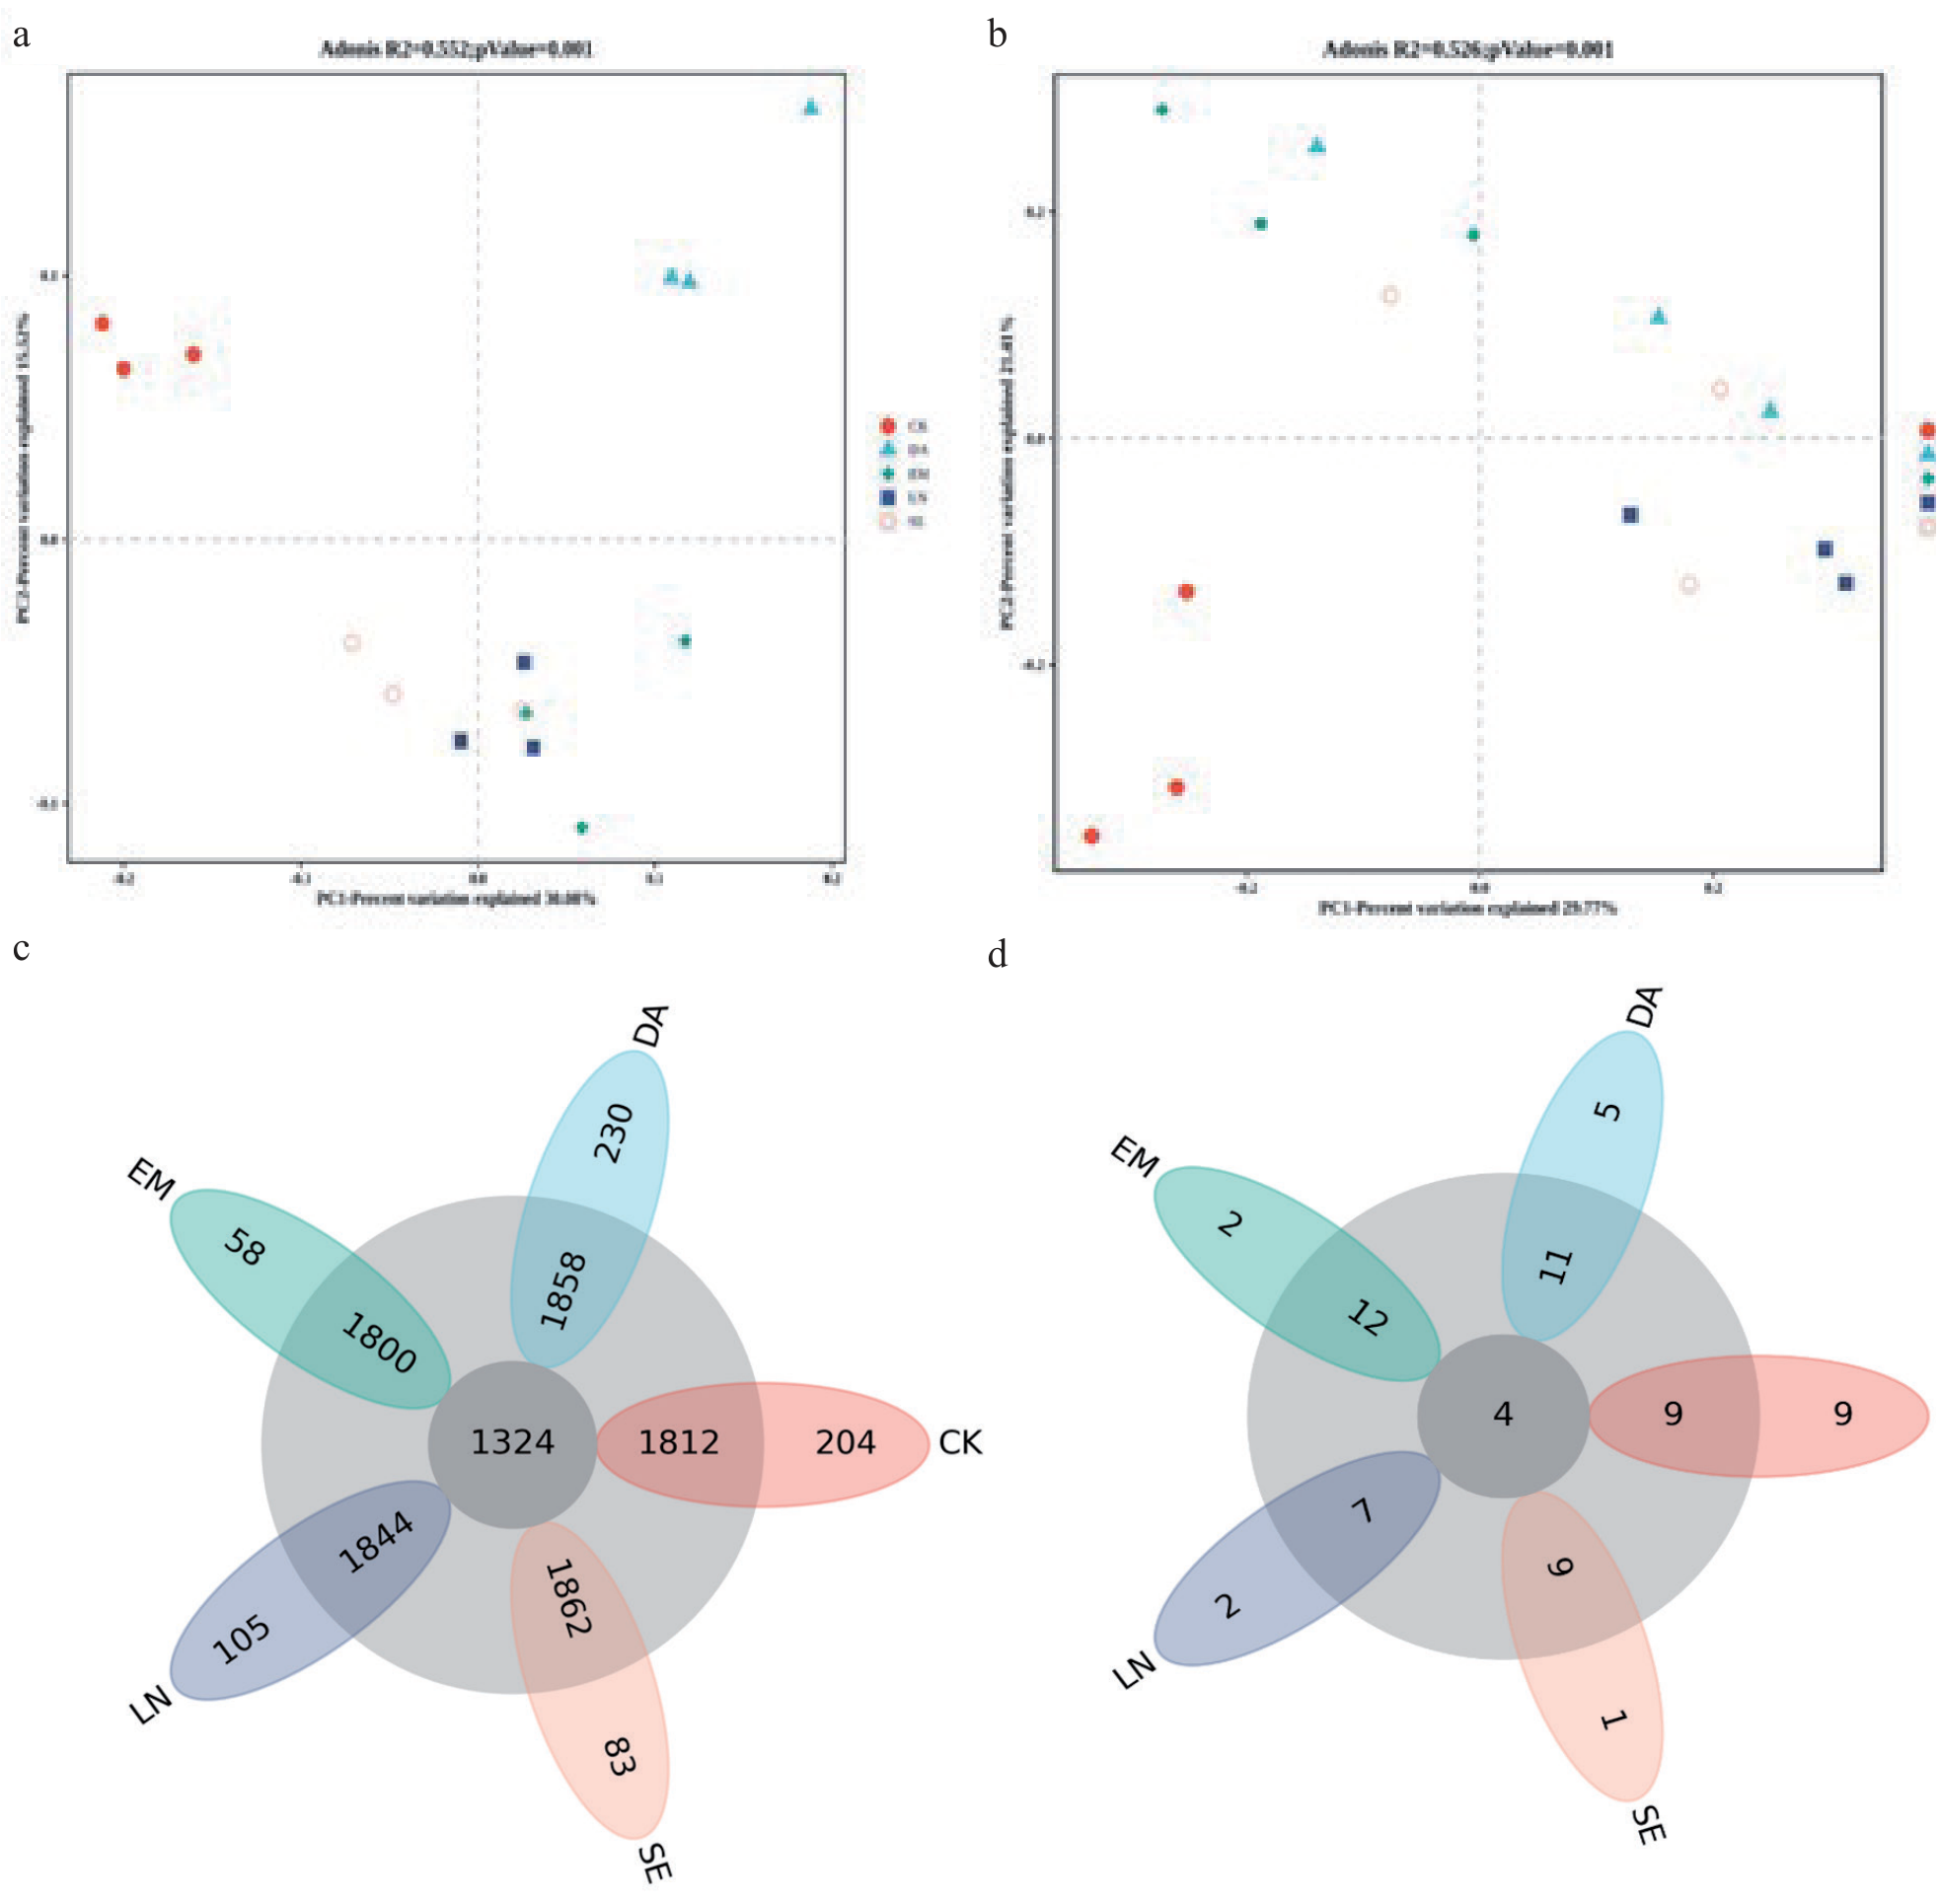
As shown in Fig. 2a, PCoA analysis of bacterial communities at the OTU level 60 days after different disinfection treatments revealed that the first and second principal coordinates accounted for 30.08% and 15.52% of the variation, respectively. The treatments were separated along the PC2 axis, with sample points for DA, EM, LN, and SE positioned farther from CK, indicating greater differences in bacterial community structures compared to the control.
As illustrated in Fig. 2b, PCoA analysis of fungal communities showed that the first and second principal coordinates explained 29.77% and 21.41% of the variation, respectively. The ANOSIM test for intergroup differences yielded an R-value of 0.526 and a p-value of 0.001. Samples from the LN, DA, and EM treatments were separated along the PC1 axis and located farther from CK, indicating more pronounced differences in fungal community composition compared with the control.
The number of common and unique microbial genera in strawberry soil after different disinfection treatments was analyzed using a Venn diagram, as shown in Fig. 2c. A total of 1324 bacterial genera were shared among all five groups, including the control (CK), indicating a common core bacterial community. Additionally, only 4 bacterial genera were found to be common and exclusive to all treatments (EM, LN, SE, DA, and CK). Additionally, 58, 105, 83, 230, and 204 bacterial genera were specific to EM, LN, SE, DA, and CK treatments, respectively. For fungi (Fig. 2d), 2, 2, 1, 5, and 9 genera were uniquely associated with EM, LN, SE, DA, and CK treatments, respectively, indicating that each disinfection method altered the microbial community structure and introduced unique microbial taxa.
Effects of Different Disinfection Methods on the Relative Abundance of Microorganisms in Strawberry Soil at the Phylum and Genus Levels
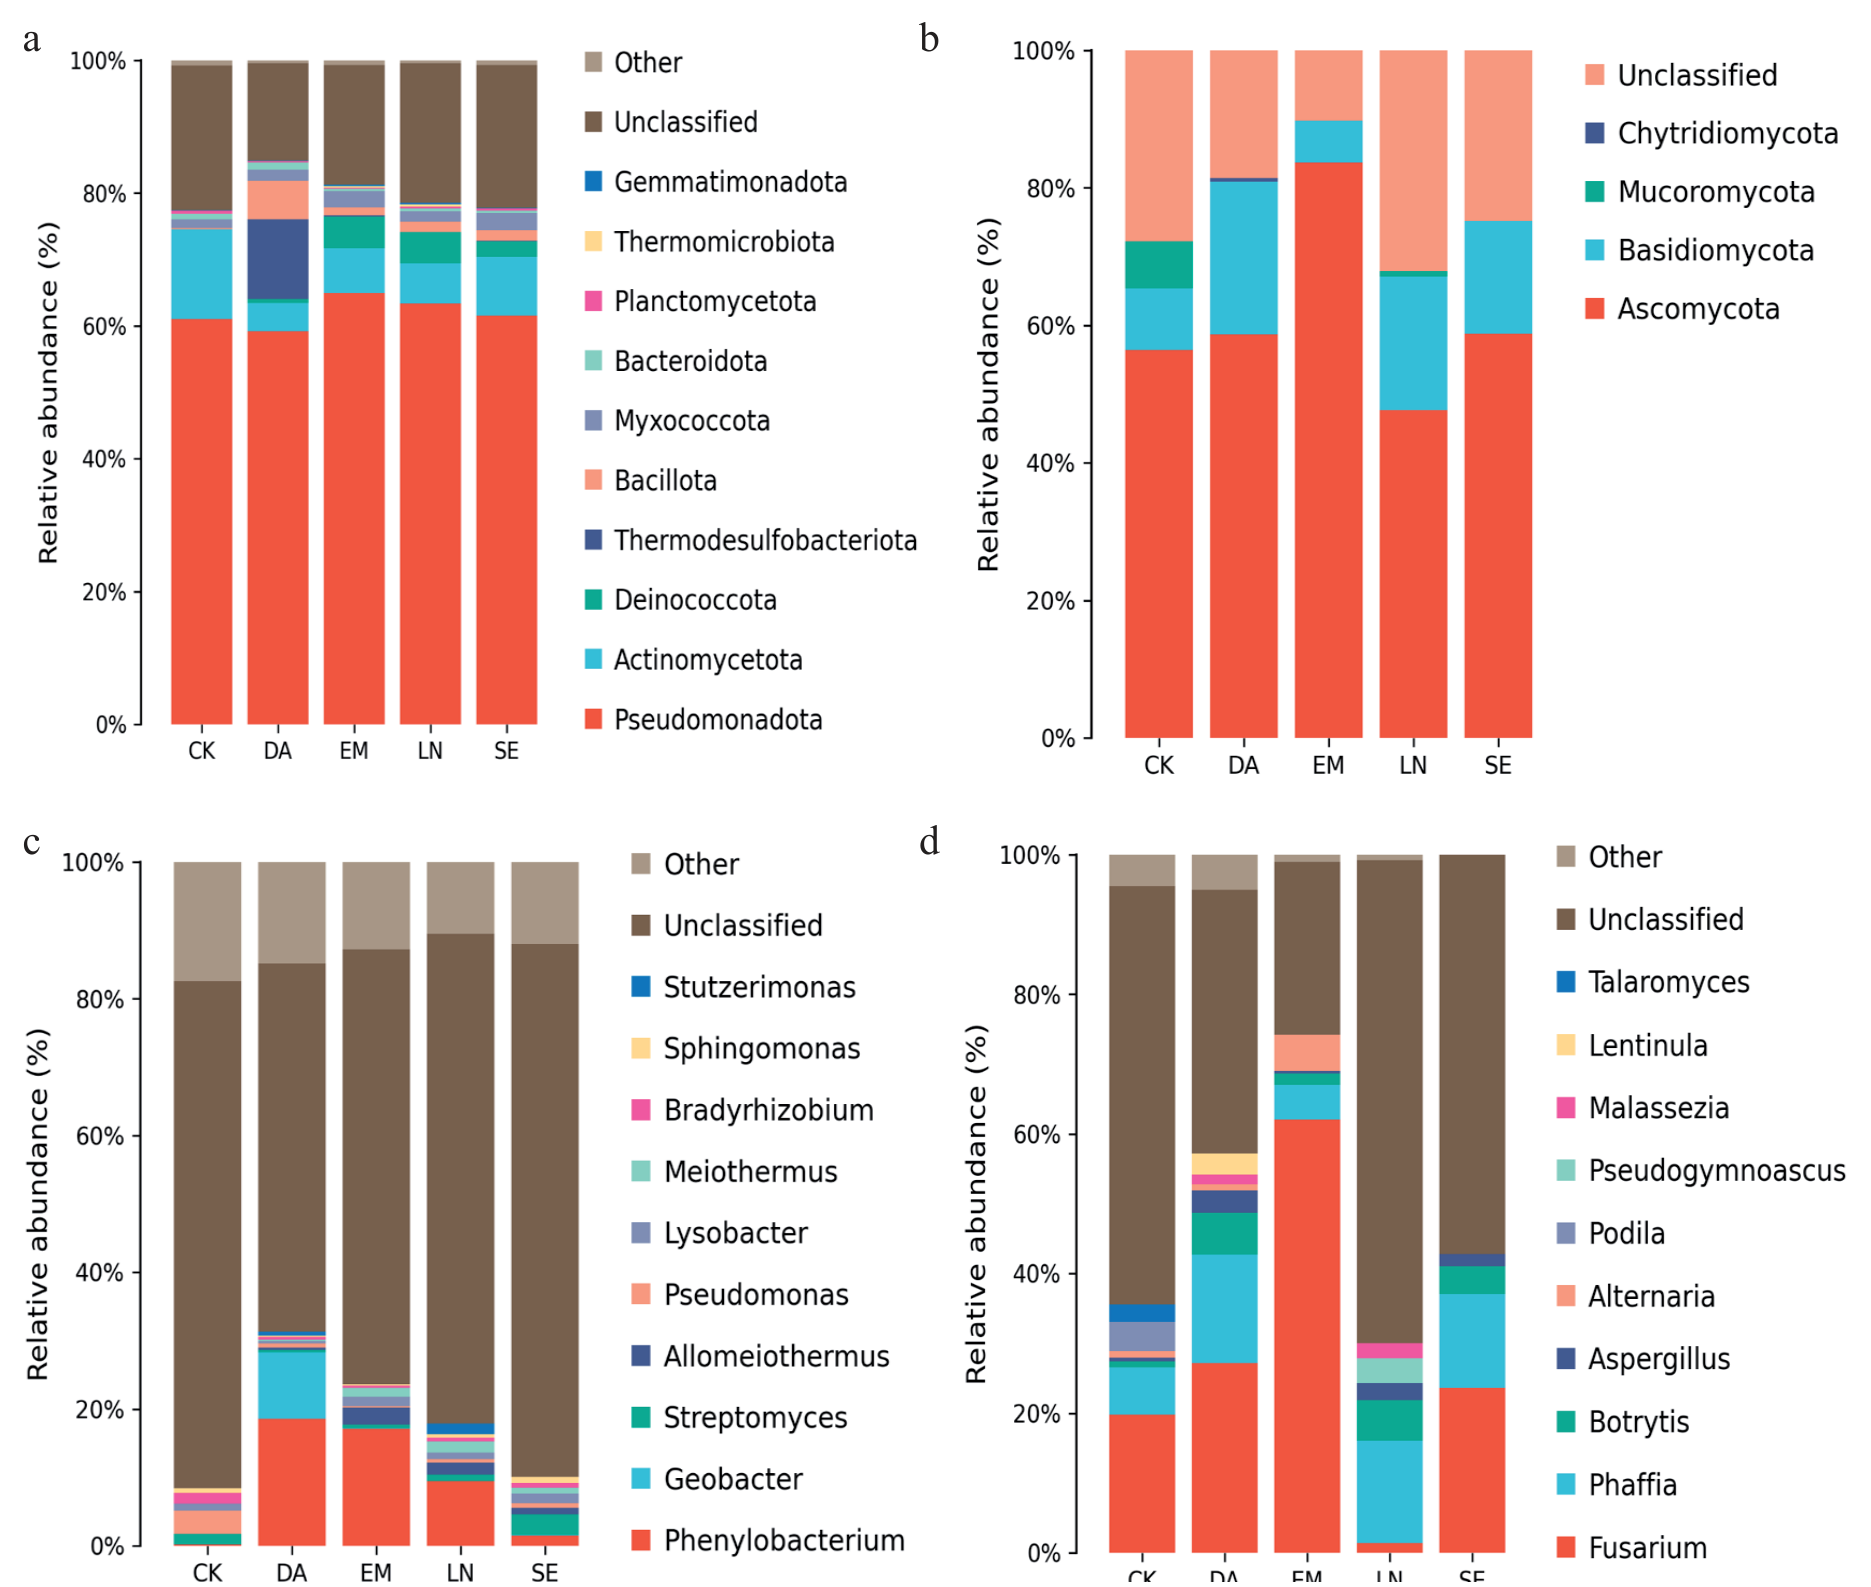
As shown in Fig. 3a, a total of 10 bacterial phyla were identified across different soil disinfection treatments, accounting for 99.15%–99.77% of total relative abundance. The five dominant phyla were Pseudomonadota, Actinomycetota, Deinococcota, Thermodesulfobacteriota, and Bacillota.
The relative abundance of Pseudomonadota followed the order EM > LN > SE > CK > DA, with increases of 3.94%, 2.34%, and 0.57% in EM, LN, and SE, respectively, compared to CK, though not statistically significant. Actinomycetota was most abundant in CK, followed by SE, EM, LN, and DA. Compared to CK, its abundance significantly decreased by 4.72%, 6.74%, 7.42%, and 9.32% in SE, EM, LN, and DA treatments, respectively (p < 0.01). The relative abundance of Deinococcota increased significantly (p < 0.01) in all treatments compared to CK, with increases of 4.73% (EM), 4.62% (LN), 2.34% (SE), and 0.64% (DA). Bacillota and Myxococcota also showed increased abundance under all treatments compared with CK, although differences were not significant.
As shown in Fig. 3c, the dominant bacterial genera were Phenylobacterium, Geobacter, Streptomyces, and Allomeiothermus, along with others (10.54%–17.44%). Phenylobacterium abundance was ranked DA > EM > LN > SE > CK, with increases of 18.42% (DA), 16.96% (EM), 9.29% (LN, p < 0.05), and 1.35% (SE) over CK. Allomeiothermus increased by 0.34%, 2.48%, 1.75%, and 0.88% in DA, EM, LN, and SE, respectively, compared to CK. Geobacter abundance increased significantly by 9.75% in DA (p < 0.05). Streptomyces was most abundant in the SE treatment, showing a 1.55% increase over CK. Meiothermus abundance increased significantly in all treatments (p < 0.01), while Sphingomonas decreased significantly (p < 0.05).
Fig. 1.
Effect of different disinfection methods on Alpha diversity of soil bacteria and fungi in continuous cropping.
As shown in Fig. 3b, dominant fungal phyla were Ascomycota, Basidiomycota, and Mucoromycota. Ascomycota abundance followed the trend EM > SE > DA > CK > LN. Basidiomycota was most abundant in DA, followed by LN, SE, CK, and EM. Compared to CK, Basidiomycota abundance increased significantly by 27.34% in DA, and by 2.38% and 2.36% in LN and SE, respectively (p < 0.05). Mucoromycota was most abundant in CK and was nearly undetectable in DA, EM, and SE, indicating a significant decrease (p < 0.001).
Fig. 2.
Effect of different disinfection methods on Beta diversity of soil bacteria and fungi in strawberry continuous cropping. a) PCoA analysis of bacterial communities; b) PCoA analysis of fungi communities; c) VENN analysis of bacterial communities; d) VENN analysis of fungi communities.
As shown in Fig. 3d, the dominant fungal genera included Fusarium, Phaffia, Botrytis, Aspergillus, Alternaria, Podila, Pseudogymnoascus, Malassezia, Lentinula, and Talaromyces, in addition to others (0.00%–7.23%). Fusarium abundance was highest in EM, followed by SE, DA, CK, and LN, with EM, SE, and DA increasing by 42.20%, 7.35%, and 3.80%, respectively, while LN showed an 18.42% decrease compared to CK. Phaffia was most abundant in DA, with increases of 8.81% (DA), 7.90% (LN), and 6.76% (SE) over CK (p < 0.05). Botrytis increased by 5.08% (DA), 5.00% (EM), and 3.09% (LN) compared to CK. Alternaria, Podila, Pseudogymnoascus, Malassezia, Lentinula, and Talaromyces were undetected in the SE treatment. Pseudogymnoascus significantly increased only in LN (p < 0.05), while Lentinula increased in DA. The relative abundance of Mucoromycota was highest in CK; DA, EM, and SE treatments significantly reduced its abundance (p<0.001), and Mucoromycota was not detected in these treatments, due to its extremely low abundance.
LEfSe Analysis of Microbial Communities
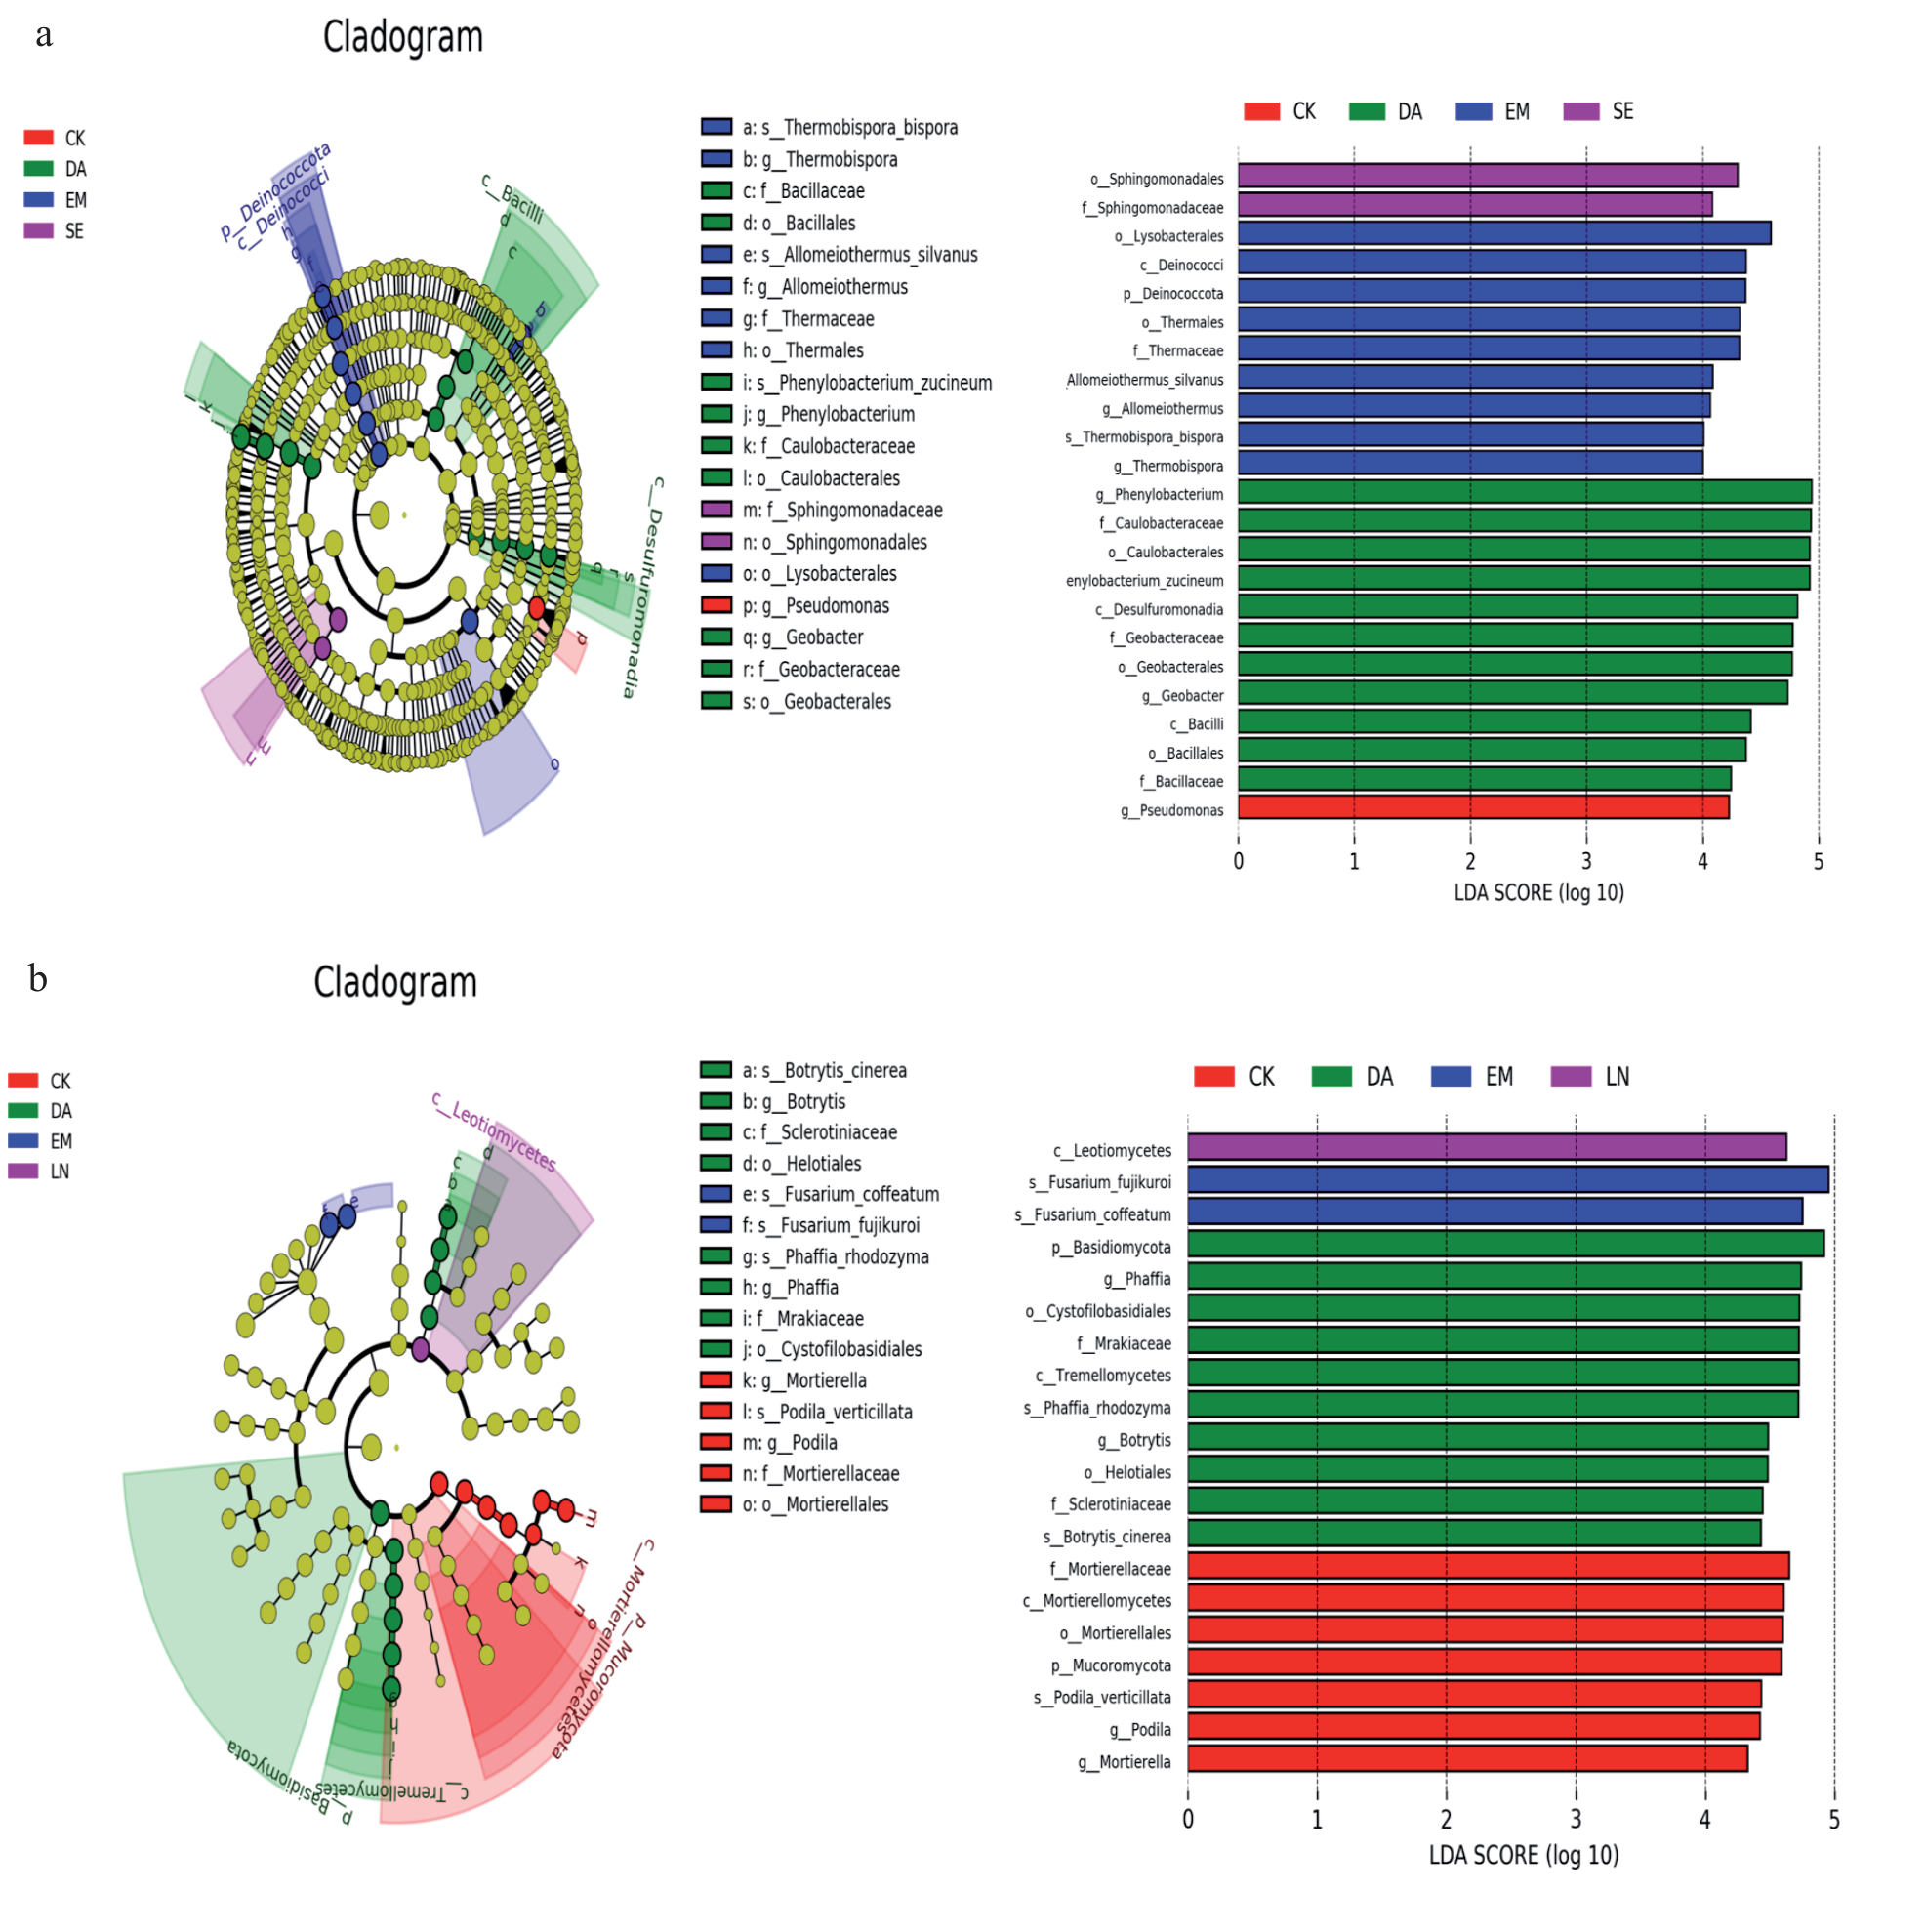
LEfSe analysis was used to identify biomarkers with significant differences among treatments at different taxonomic levels (LDA> 4, p < 0.05) (Fig. 4). A total of 23 bacterial biomarkers were identified across the different treatments and CK, with one bacterial species enriched in the CK treatment. As shown in Fig. 3a, at the LDA>4.5 level, Pseudomonas was enriched in CK. In the SE treatment, Sphingomonadales and Sphingomonadaceae were enriched. In EM, Lysobacterales, Deinococcota, Deinococci, Thermales, and Themaceae were the dominant taxa. For fungi, 19 abundant taxa differed significantly among CK, DA, EM, and LN treatments. As shown in Fig. 3b, at the LDA > 4.5 level, Mortierellaceae, Mortierellomycetes, Mucoromycota, Podila_verticillata, Podila, and Mortierella were enriched in CK. Leotiomycetes were enriched in the LN treatment. Fusarium fujikuroi and Fusarium coffeatum were enriched in EM, while Basidiomycota, Phaffia, Cystofilobasidiales, Mrakiaceae, and Tremellomycetes were enriched in DA.
Effects of Different Disinfection Methods on the Molecular Ecological Network of Microorganisms in Strawberry Inter-Root Soil
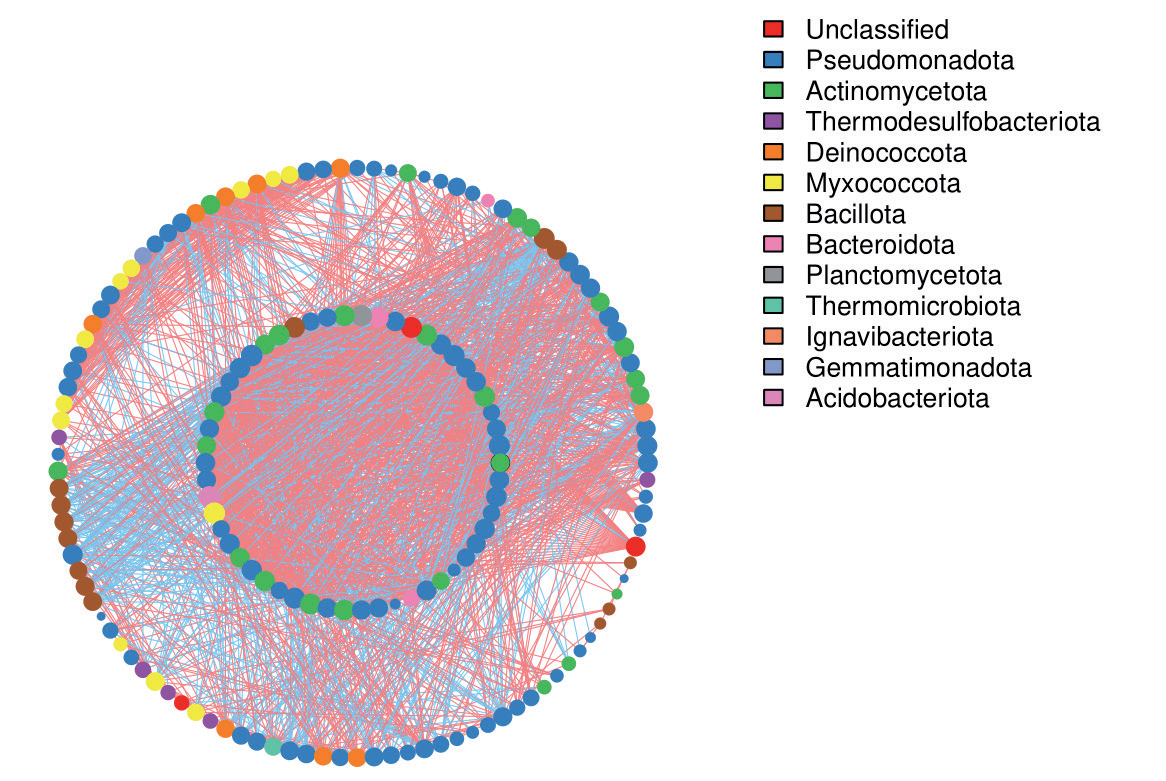
Based on bacterial sequence data from different treatments, OTUs with a relative abundance greater than 0.5% were selected to construct microbial molecular ecological network maps to analyze potential interactions between bacterial communities. Compared with the control, the number of edges in the bacterial molecular ecological networks increased after different treatments (Fig. 5), indicating enhanced network stability. The DA treatment showed a notable increase in the number of nodes, while the LN treatment showed a significant increase in the number of edges. Correlation analysis indicated that positive correlations dominated the bacterial molecular ecological networks across all treatments. The positive correlation coefficients for SE, LN, EM, and DA treatments were 55.35%, 56.95%, 55.29%, and 53.27%, respectively, suggesting enhanced synergistic interactions among bacterial communities. Moreover, the similarity of bacterial groups composing the networks across treatments was high. Key nodes in the networks were mainly associated with Presudomonadota, Actinomycetora, Thermondesulfobacteriota, Deinococcota, Bacillota, Bacteroidota, Planctomycetora, Thermomicrobiota, Ignavibacteriota, Gemmatimonadota, and Acidobacteriota.
Redundancy Effects of Different Sterilization Methods on Strawberry Inter-Root Soil Microorganisms and Meta-Analysis
To further investigate the relationship between different soil disinfection methods on the dominant species of strawberry inter-root microbial communities, redundancy analysis was performed using soil physicochemical factors. The results showed that the RDA1 and RDA2 axes explained 43.92% and 28.54% of the variation in soil bacterial communities across different disinfection methods, respectively (Fig. 6a). For fungal communities at the genus level, the RDA1 and RDA2 axes explained 36.18% and 16.83%, respectively.
Soil OC, RVP, UR, and pH were significantly and positively correlated with phenylob, Allomeiothermus, and Meiothermus. Soil CA and AP were significantly and positively correlated with Streptom, Sphigomonas, and Bradyrhizobium (Fig. 6b). Soil EC, RVP, NP, OC, and TN were significantly and positively correlated with Stutzerimonas and Geobacter. Soil CA, AP, and pH showed significant negative correlations with Stutzerimonsa and Geobacter. Soil NP, SU, and AP were significantly and negatively correlated with Allomeiothermus and Meiothermus. Soil RVP, EC, and NP were significantly and negatively correlated with Streptomyces and Sphingomonas. Soil OC, TN, and RVP were significantly and negatively correlated with Pseudomonas.
Fig. 5.
Effects of different disinfection methods on the molecular ecological network of microorganisms in strawberry inter-root soil
Soil NP, AP, and SU were significantly and positively correlated with Podila, Altermaria, and Fusarium. Soil NP, AP, and EC were significantly and positively correlated with Talaromyces. Soil EC, RVP, and TN were significantly and positively correlated with Lentinula, Aspergillus, and Malassezia. Soil TN, OC, pH, and CA were significantly and positively correlated with Pseudogmonas, Phaffia, and Botrytis. Soil OC, CA, pH, UR, and TN were significantly and negatively correlated with Talaromyces and Podila. Soil TN, RVP, OC, pH, and CA were significantly and negatively correlated with Alternaria and Fusarium. Soil SU, AP, and NP were significantly and negatively correlated with Malassezia, Aspergillus, Phaffia, and Botrytis.
Fig. 6.
RDA analysis of soil physicochemical properties and microbial diversity. a) bacteria communities; b): fungi communities A: RDA analysis of soil bacterial communities and environmental factors; B: RDA analysis of soil fungi communities and environmental factors; C: Meta-analysis of s of soil bacterial communities and environmental factors ; D: Meta-analysis of soil fungi communities and environmental factors.Note: phenylob: Phenylobacterium; Allomeio: Allomeiothermus; Meiother: Meiothermus; Lysobact: Lysobacter; Sreptom: Streptomyces; Sphingom: Sphingomonas; Bradythz: Bradyrhizobium; Pseudomn: Pseudomonas; Geobactr: Geobacter; Stuzerm: Stutzerimonas. Podila: Altemar: Alternaria; Pseudogm: Pseudomonas; Aspergil: Aspergillus; Malassez: Malassezia; Lentinul: Lentinula; Talarome: Talaromyces. EC: TN: Total nitrogen; AP: Available phosphorus; RVP: Available phosphorus; OC: Organic carbon; UR: Urease; CA: Catalase; SU: Sucrase; NP: Neutral phosphatase.
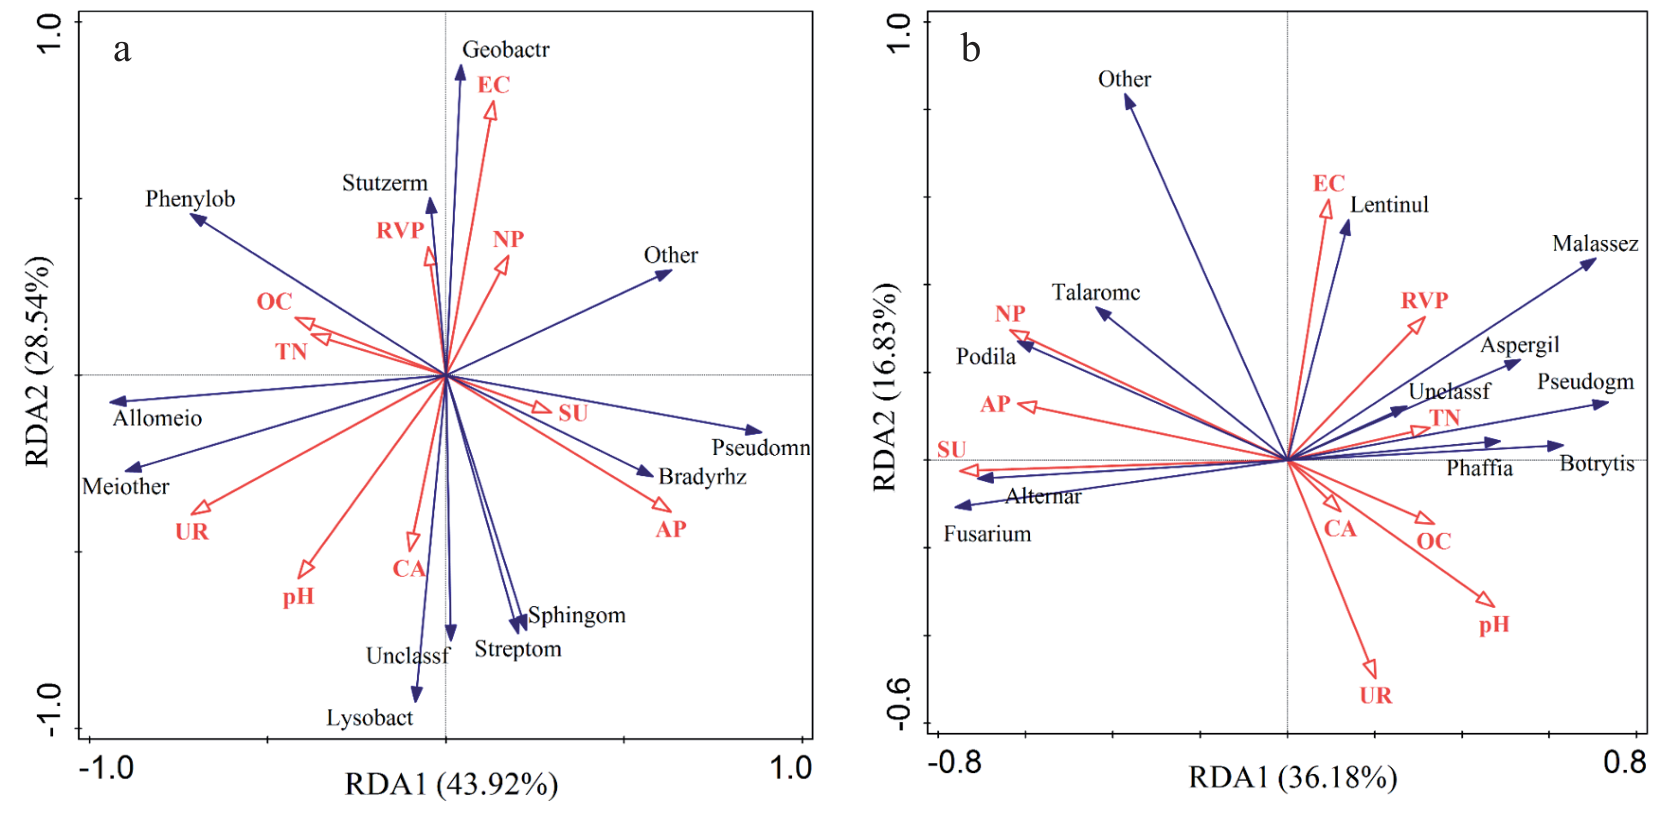
Fig. 7.
Correlation analysis of soil physicochemical properties and microbial diversity. a) bacteria communities; b) fungi communities
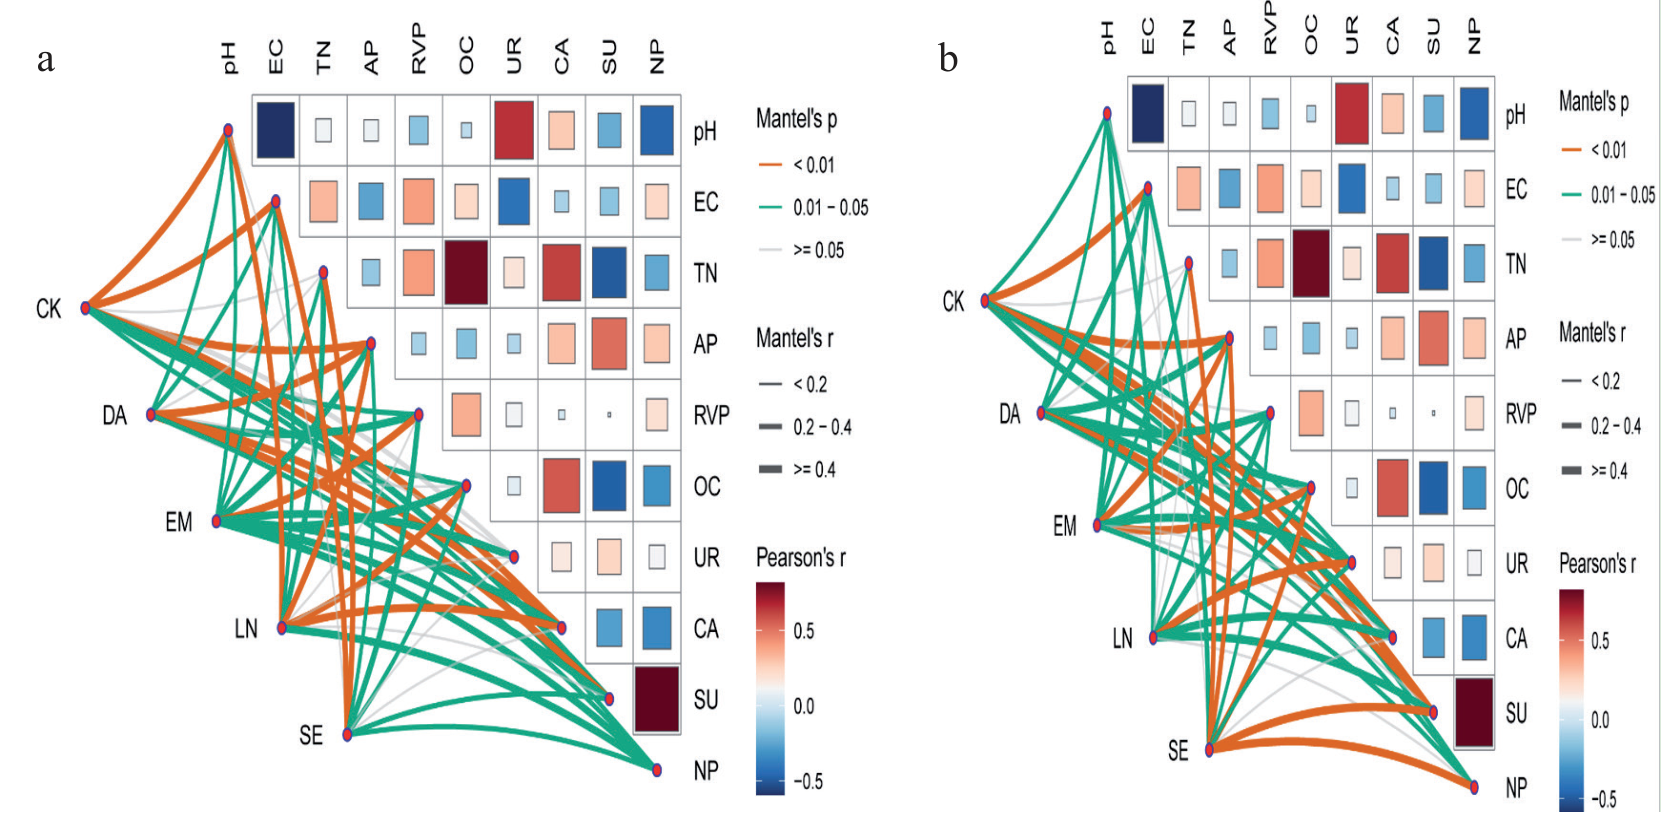
The Mantel test results (Fig. 7a) revealed significant shifts in the soil bacterial and fungal community structures under different treatments compared to the control. In the control (CK), microbial communities were primarily shaped by soil pH, EC, AP, OC, UR, CA, SU, and NP, with TN and RVP exerting limited influence.
Across the treatments (DA, EM, LN, SE), the number and identity of influential soil factors varied, indicating treatment-specific microbial responses. Notably, AP (available phosphorus), OC (organic carbon), UR (urease activity), and NP (nitrate) emerged as consistent drivers of bacterial community changes under all treatments, though their relative importance differed. pH and EC remained key influencers in most treatments, especially in DA and EM, but lost significance in SE.
For fungal communities (Fig, 7b), a broader sensitivity to soil factors was observed. While CK fungal composition was shaped by most factors except TN, EM, and LN treatments showed the strongest overall correlations, with all measured variables exerting significant effects. In contrast, SE treatment showed a narrowed response, with the fungal community influenced mainly by EC, TN, AP, OC, CA, and NP.
Overall, AP, OC, and NP were among the most consistently influential factors across microbial communities, while the strength and direction of pH and EC effects varied with treatment. These findings underscore the differential sensitivity of microbial communities to soil physicochemical properties under distinct fertilization regimes.
Effect of Different Soil Sterilization Methods on Metabolic Functions of Soil Microbial Communities
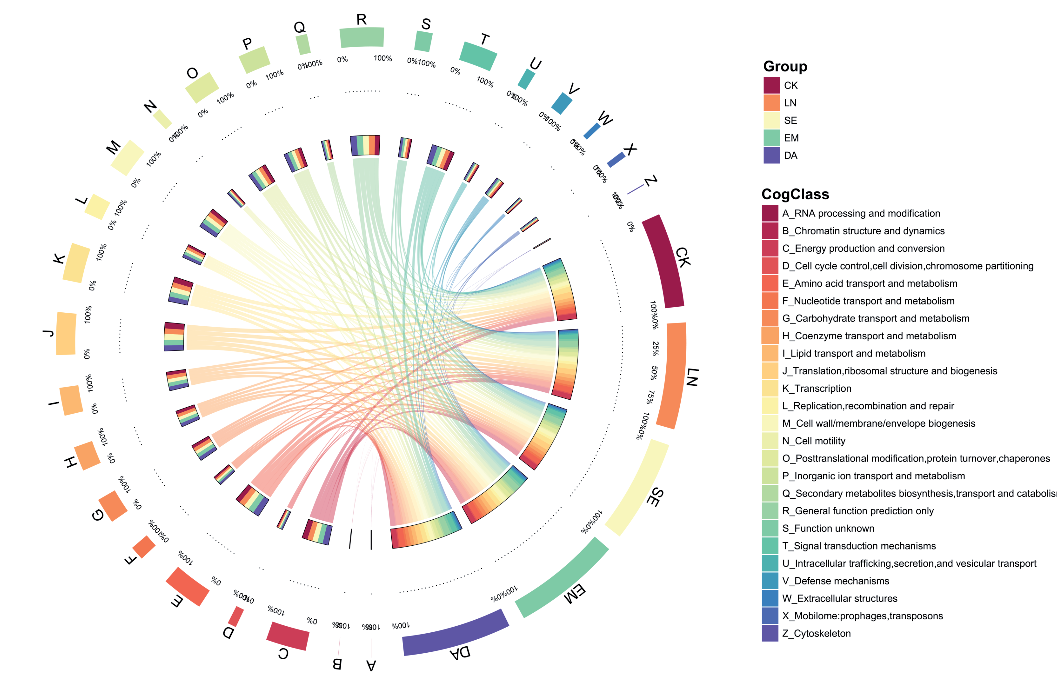
Functional categorization based on EggNOG annotations revealed that 50% of microbial functions across treatments were related to metabolism (Fig. 8). Among these, energy production and conversion was the most abundant category, followed by carbohydrate transport and metabolism, and amino acid transport and metabolism.
Energy production and conversion accounted for 19.79%, 19.61%, 19.71%, 19.75%, and 21.13% in the CK, LN, SE, EM, and DA treatments, respectively. Carbohydrate transport and metabolism accounted for 16.46%, 21.66%, 18.48%, 22.40% and 21.00% in the CK, LN, SE, EM, and DA treatments, respectively. Signal transduction mechanisms accounted for 18.26%, 19.43%, 19.52%, 19.86%, and 22.93%, while replication, reorganization, and repair accounted for 16.21%, 16.21%, 19.11%, 19.68%, and 22.00% in the respective treatments. Different sterilization methods increased the relative abundance of functions related to amino acid transport and metabolism, carbohydrate transport and metabolism, and replication, recombination, and repair, but decreased functions related to RNA processing and modification, transcription, and the cytoskeleton.
Table 2.
Effects of different soil sterilization methods on soil enzyme activity of continuous cropping soil.
Effects of Different Soil Sterilization Methods on Soil Enzyme Activity of Continuous Cropping Soil
As shown in the Table 2, soil urease activity increased significantly by 48.15%, 32.00%, and 8.13% in the LN, EM, and DA treatments, respectively, compared to CK, and decreased significantly by 12.56% (p<0.05) in the SE treatment. There were no significant differences in soil catalase activity among the treatments compared to CK. Soil sucrase and neutral phosphatase activities increased significantly by 7.88% and 9.68% (p<0.05), respectively, in the LN treatment. Soil sucrase activity decreased significantly by 21.86%, 36.38%, and 27.24% (p<0.05) in the SE, EM, and DA treatments, respectively, compared to CK. Soil neutral phosphatase activity decreased by 0.54%, 20.43% (p<0.05), and 18.28% (p<0.05) in the SE, EM, and DA treatments, respectively, compared to CK.
Discussion
Selective nutrient uptake by the same crop can lead to soil nutrient depletion, while irrational application of chemical fertilizers can cause salt accumulation and soil pH abnormalities during continuous cropping [19]. In practice, measures such as soil disinfection, rational crop rotation, and the selection of resistant varieties are commonly used to alleviate continuous cropping disorders [20]. Studies have shown that disinfectants can inhibit soil-borne diseases; however, disinfectants and their degradation products may have a negative impact on soil microbial communities and the soil environment [21]. The significant decrease in soil pH observed in the DA treatment in this study may be attributed to the hydrolysis of methyl isothiocyanate, produced by the decomposition of dazomet, which generates corresponding acids. These acids increase the hydrogen ion concentration, thereby contributing to the decline in soil pH. In addition, soil disinfection with dazomet can kill microorganisms crucial for maintaining the soil's acid-base balance, disrupting the original equilibrium and further lowering the soil pH. The significant increase in soil electrical conductivity (EC) observed in the DA treatment (+42.29%, p < 0.05) suggests a notable accumulation of soluble salts, likely resulting from the application of chemical fertilizers that contain readily available ionic forms of nutrients such as nitrate, ammonium, and potassium. This elevation in EC may have implications for soil osmotic potential, potentially affecting root water uptake and plant physiological responses under prolonged exposure.
Soil microorganisms, as key components of the soil ecosystem, play critical roles in nutrient cycling and organic matter mineralization [22, 23]. Research has demonstrated that crop succession significantly alters the composition and abundance of soil microbial communities, often resulting in an imbalance characterized by a shift from bacterial to fungal dominance, which in turn affects nutrient cycling [24]. Li et al. (2021) reported that microbial fumigation significantly increased the abundance and diversity of the soil bacterial community in tomato succession soils [25]. Similarly, Liang et al. (2021) found that continuous application of organic amendments significantly improved soil quality and enhanced microbial metabolic activity [26]. Therefore, adopting effective strategies to regulate soil microbial community structure is critical for alleviating continuous cropping disorders. Based on α- and β-diversity analyses, including specific assemblages and functional predictions, we found that microbial community richness and diversity decreased following different soil disinfection treatments in continuously cropped strawberry soils, consistent with previous findings [27]. Different soil disinfection methods significantly affected bacterial phylum abundance and uniformly reduced the relative abundance of Actinomycetes. Dazomet disinfection releases toxic substances that nonspecifically kill soil microorganisms, making Actinomycetes vulnerable. High-temperature disinfection methods, such as solarization, cause rapid increases in soil temperature that can damage actinomycete cell structures and biomolecules. Lime nitrogen disinfection elevates soil pH, potentially pushing conditions outside the optimal survival range for Actinomycetes. DA treatment significantly increased the relative abundance of Thermodesulfobacteriota, a phylum of thermophilic sulfate-reducing bacteria. Microorganisms within the Thermodesulfobacteriota phylum may adapt to environmental changes induced by dazomet decomposition. For instance, hydrogen sulfide production may supply sulfur to sulfur-metabolizing microorganisms such as B. thermodesulfuricans, promoting their growth and reproduction. Furthermore, the accelerated decomposition of organic matter following dazomet disinfection releases more nutrients, which may also favor the proliferation of Thermodesulfobacteriota microorganisms.
The top three dominant fungal phyla in soils subjected to different disinfection treatments were Ascomycota and Basidiomycota. The DA, EM, and SE treatments had the most significant effect on reducing the relative abundance of Mucoromycota (P<0.001), and no Mucoromycota were detected in soil samples from these treatments. Ascomycota has been reported to promote nutrient uptake by plant roots and support plant growth and development. Compared with other disinfection methods, DA, LN, and SE significantly increased the relative abundance of Trichoderma (Ascomycota) and were significantly and positively correlated with organic matter content and catalase activity. Thus, DA, LN, and SE enhanced the number of beneficial microorganisms and optimized the soil microenvironment. In this study, the abundance of Bacillus and Thick-walled bacteria significantly increased in soils treated with dazomet compared to the control. Studies have shown that most Bacillus species produce beneficial substances such as phytohormones and antibiotics, which regulate plant growth [28]. Thick-walled bacteria promote organic matter decomposition and play an essential role in soil ecosystem cycling [29]. At the fungal level, DA and SE treatments increased the relative abundance of Ascomycota. Ascomycetes favor the decomposition of organic materials such as leaves and wood debris [30]. Additionally, DA and SE treatments increased the relative abundance of the beneficial fungal genus Stachybotrys.
Soil enzyme activity, a key indicator of soil health, mainly reflects microbial metabolism and nutrient cycling processes [31]. Soil sucrase hydrolyzes sucrose into monosaccharides, providing nutrients for microorganisms and influencing organic carbon mineralization. Catalase decomposes hydrogen peroxide, reducing its toxicity. Urease hydrolyzes urea and increases inorganic nitrogen content. These three enzymes are representative indicators of soil enzyme activity, crucial for evaluating soil fertility and ecological status [32]. This study showed that dazomet disinfection decreased soil sucrase and neutral phosphatase activities, likely due to the reduction of microorganisms responsible for these enzyme activities. LN treatment increased the activities of urease, sucrase, and neutral phosphatase, while EM treatment enhanced urease and sucrase activities, improving soil fertility to some extent. Previous studies reported that microbial fumigation significantly increased soil urease and polyphenol oxidase activities after straw return [33], which aligns with our findings. It has also been shown that applying organic amendments after fumigation stimulates microbial metabolism but depletes soil nutrients, resulting in decreased effective phosphorus, potassium, and organic matter content [34].
Conclusions
(1) EM treatment reduced soil pH, conductivity, and available phosphorus content, which may improve strawberry quality and promote plant growth. These findings suggest that EM-associated beneficial microorganisms can alter the micro-ecological environment and regulate soil nutrient and material transportation.
(2) All treatments reduced bacterial and fungal diversity and abundance to varying degrees, with EM treatment significantly affecting bacterial diversity and LN treatment significantly affecting fungal diversity. Dazomet fumigation notably increased the relative abundance of beneficial bacteria in the genera Bacillariophyta and Thick-walled Bacteria.
(3) All disinfection treatments, except LN, increased the relative abundance of Ascomycota, indicating that soil disinfection could favor organic matter decomposition. Changes in physicochemical properties such as pH, total nitrogen, RVP, OC, UR, SU, and NP were important factors influencing microbial community shifts in disinfected continuous cropping strawberry soils.
(4) EM treatment improved soil fertility by increasing urease and sucrase activities. Meanwhile, it reduced soil pH, conductivity, and available phosphorus content, suggesting that EM-associated beneficial microorganisms can modify the micro-ecological environment and regulate soil nutrient and material cycling processes.
(5) Different treatments increased the complexity of the soil bacterial molecular ecological network and improved the stability of the bacterial community, with higher network stability observed after DA and LN treatments. KEGG functional predictions revealed that disinfection treatments increased the relative abundance of functions related to amino acid transport and metabolism, carbohydrate transport and metabolism, as well as replication, recombination, and repair. DA and EM treatments were particularly effective in regulating the soil microbial community and promoting soil material cycling.

