

Introduction
Tea plants (Camellia sinensis (L.) O. Kuntze) represent a significant woody economic plant widely cultivated worldwide [1]. However, the widespread practice of large-scale monoculture in tea cultivation has led to a considerable reduction in soil microbial diversity and an increase in disease prevalence, adversely impacting both yield and quality of tea [2, 3]. To mitigate these issues, the construction of multi-layered and ecological tea gardens incorporating intercropping systems is gaining recognition as a vital agricultural strategy. The intercropping system not only directly enhances soil fertility but also achieves ecological optimization via comprehensive effects, including improved canopy microclimate and amplified biodiversity, ultimately elevating tea yield and quality constituents [4]. This ecological intensification mechanism originates from resource complementarity effects between tea plants and intercrops, whereby interspecific interactions govern tea plants’ acquisition and utilization efficiency of hydrological resources, soil nutrients (nitrogen, phosphorus, potassium), and photosynthetically active radiation, thereby systematically modulating vegetative growth, phytochemical profiles, and productivity outcomes [5]. Studies indicate that different intercropping patterns can positively affect the formation of tea quality. Notably, changes in shading and light conditions associated with intercropping significantly affect the internal metabolic processes of tea plants, leading to an increase in amino acid content and a reduction in catechin content, thereby improving tea quality [6]. For instance, a study conducted in southern Shaanxi, China, demonstrated that intercropping pine trees with tea plants, as opposed to using plastic shade or practicing monoculture, resulted in significant increase in amino acid and water extract content of tea leaves, while simultaneously reducing tea polyphenol levels and thereby substantially optimizing tea quality [7]. In light of these findings, a deeper understanding of the mechanisms underlying the benefits of intercropping is essential for improving intercropping combinations and cultivation practices, thereby offering effective solutions to the challenges posed by monoculture in tea cultivation.
As investigations into the benefits of intercropping continue to evolve, numerous scholars have observed that, under complex planting conditions, changes in soil microbial community structure and increased diversity are closely related to soil enzyme activity, nutrient cycling, and the plants’ resilience to biotic and abiotic stress [8]. The nutrient cycling and energy flow processes mediated by soil microbes lead to changes in the soil ecological environment, which in turn influence plant growth [9, 10]. The study by Wu [11]demonstrated that the increases in soil organic matter (SOM), available phosphorus (AP), and available potassium (AK) in the tea plant and chestnut intercropping system exhibited positive correlations with microbial communities such as Chloroflexi, WPS-2, and Bacteroidota, which enhance the soil nutrient acquisition capacity of tea plants. Research by Bai [12] revealed that tea plants improved soil nutrient status and enzyme activity in tea gardens through intercropping with walnut, while simultaneously elevating the operational taxonomic unit (OTU) abundance associated with nutrient cycling, disease prevention, and improved abiotic stress tolerance functions. Furthermore, the study by Zhong [13] indicated that tea intercropping with soybean and rapeseed not only significantly increased the relative abundance of potentially beneficial bacteria related to essential mineral nutrient cycling for tea plants but also markedly enhanced soil microbial functions associated with nutrient cycling processes.
Although the response mechanisms of soil microbial community structures to intercropping are not fully understood, the enrichment of beneficial microbial communities in these systems provides valuable evidence for alleviating continuous cropping obstacles, making the assessment of soil microorganisms under intercropping conditions essential for addressing continuous cropping issues in tea cultivation.
In choosing companion crops for tea plants, bamboo fungus (Dictyophora indusiata (Vent ex Pers) Fisch.), a precious edible and medicinal fungus from the family Phallaceae, is recognized for its rich nutrient profile [14]. Bamboo fungus, as a saprophytic fungus, relies on the decomposition of organic matter for its growth rather than competing with tea plants for mineral nutrients. Furthermore, its vertically growing fruiting body structure minimizes competition for light resources. Research indicates that intercropping bamboo fungus can effectively utilize understory space resources, regulate sugarcane root development, and promote nutrient transport [15]. Therefore, while intercropping bamboo fungus holds the potential to promote soil nutrient cycling within tea gardens, there remains a paucity of research investigating the tea plant/bamboo fungus intercropping system. To address this gap, the present study designated bamboo fungus as an intercropping species within tea gardens, monitoring changes in soil moisture content and physicochemical properties while analyzing the soil microbial community through high-throughput sequencing techniques. The study aimed to assess the impact of monoculture versus bamboo fungus intercropping on the composition, structure, and function of microbial communities within tea plant soil, with the findings providing valuable insights into the structure and functional response mechanisms of these communities in tea gardens intercropped with bamboo fungus, thereby providing theoretical support for the construction of modern ecological composite tea gardens.
Experimental
Experimental Site Overview
The experiment was conducted in the tea garden located at Ting Village, Jianyang District, Nanping City, Fujian Province (118º06′13″E, 27º13′48″N). The region has a subtropical monsoon humid climate, with an average annual sunshine duration of 1629.5 hours and average annual precipitation of 1926.9 mm. The tea garden features an inter-row spacing of 1 meter, and the tea plants used for the experiment were five-year-old Camellia sinensis L. cv. Rougui.
Experimental Design
Two treatments were randomly assigned: intercropping (IN) and monoculture (CK). In January 2022, bamboo fungus was planted in the middle of the tea rows, maintaining a distance of 0.5 meters from both sides of the tea plants. Cultivation management practices were consistent across both treatments, employing manual weeding and avoiding the use of chemical herbicides or insecticides. Additionally, a compound fertilizer with a nutrient ratio of N: P: K = 21:8:16 was applied annually at a rate of 700 kg/ha each October.
Soil Sample Collection
Following the research methods proposed by Zhong [16], soil samples were collected in mid-May 2023 on a clear day (ambient temperature 20-25ºC). Five biological replicates were established for each treatment. A standard five-point sampling method was used to obtain soil samples for each replicate. Sampling was performed at a depth of 10-20 cm using a sterilized stainless steel soil corer (diameter 5 cm), after removing the surface litter (0-5 cm) to exclude undecomposed organic matter. Visible roots and gravel (>2 mm) were manually removed from the collected soil. Each sample was homogenized using the quartering method and then divided into two parallel portions: one portion was air-dried at 25ºC for 72 hours, ground with a mortar and pestle, and sieved through a 100-mesh nylon sieve for soil nutrient index determination; the other portion was immediately aliquoted into sterile cryovials and stored at -80ºC for subsequent DNA extraction experiments. Samples were transported to the laboratory within 2 hours in an insulated box (4ºC).
Soil Physicochemical Properties Measurement
Soil pH was measured using the potentiometric method. Soil saturated water content (SM), field water-holding capacity (FC), soil capillary water-holding capacity (SCC), total porosity (TP), and soil bulk density (BD) were determined using the ring knife method. Soil moisture content (MC) was measured by the drying method. Soil organic carbon (SOC) and soil organic matter (SOM) were measured using the potassium dichromate oxidation-heating method. Alkaline nitrogen (AN) was determined using the alkaline hydrolysis diffusion method. Available phosphorus (AP) was measured using the molybdenum-antimony colorimetric method, while available potassium (AK) was measured by the flame photometry method.
Total Soil DNA Extraction
Soil total DNA was extracted using the BioFast Soil Genomic DNA Extraction Kit (BioFlux, Hangzhou, China). DNA purity was assessed using 1% agarose gel electrophoresis, while the concentration was measured using a NanoDrop2000C Spectrophotometer (Thermo Scientific, Massachusetts, USA). DNA of adequate quality was subsequently used for high-throughput sequencing analysis of the microbial community.
16S rDNA High-Throughput Sequencing Analysis
The 16S rDNA from the soil samples was amplified using an ABI GeneAmp® 9700 PCR system. The soil microbial DNA was then sequenced on the Illumina HiSeq sequencing platform. Raw data generated from the next-generation sequencing conducted on the Illumina MiSeq platform were analyzed using the QIIME2 (Quantitative Insights Into Microbial Ecology 2) Linux platform. Specifically, the q2-demux and q2-cutadapt trim-pair methods were used to remove barcodes and linker sequences. Vsearch software was used to merge the sequences. Quality control was performed using the quality-filter and deblur plugins in QIIME2, ensuring a quality score greater than 25, followed by denoising. Operational taxonomic units (OTUs) were clustered at a 97% sequence similarity threshold, and annotation was performed using the SILVA(v138) database with the q2-feature-classifier plugin.
Data Analysis
The physicochemical data of the tea soil were initially organized using Microsoft Office 2021 and analyzed for significance using ANOVA and the LSD test (p<0.05) with IBM SPSS (version 26). Soil microbial community diversity indices were plotted with GraphPad Prism (version 7.0). Principal component analysis (PCA) was performed to assess the overall differences in soil bacterial community structure. The “igraph” package in R software (version 4.3) was used to calculate the symbiotic network (Spearman, r>0.7, p<0.01), which was then visualized using Gephi (version 0.9.7) and Cytoscape (version 3.9.1). Functional annotation of the soil bacterial community was performed using the FAPROTAX database.
Results and Discussion
Effects of Intercropping on Soil Physicochemical Properties of Tea Plants
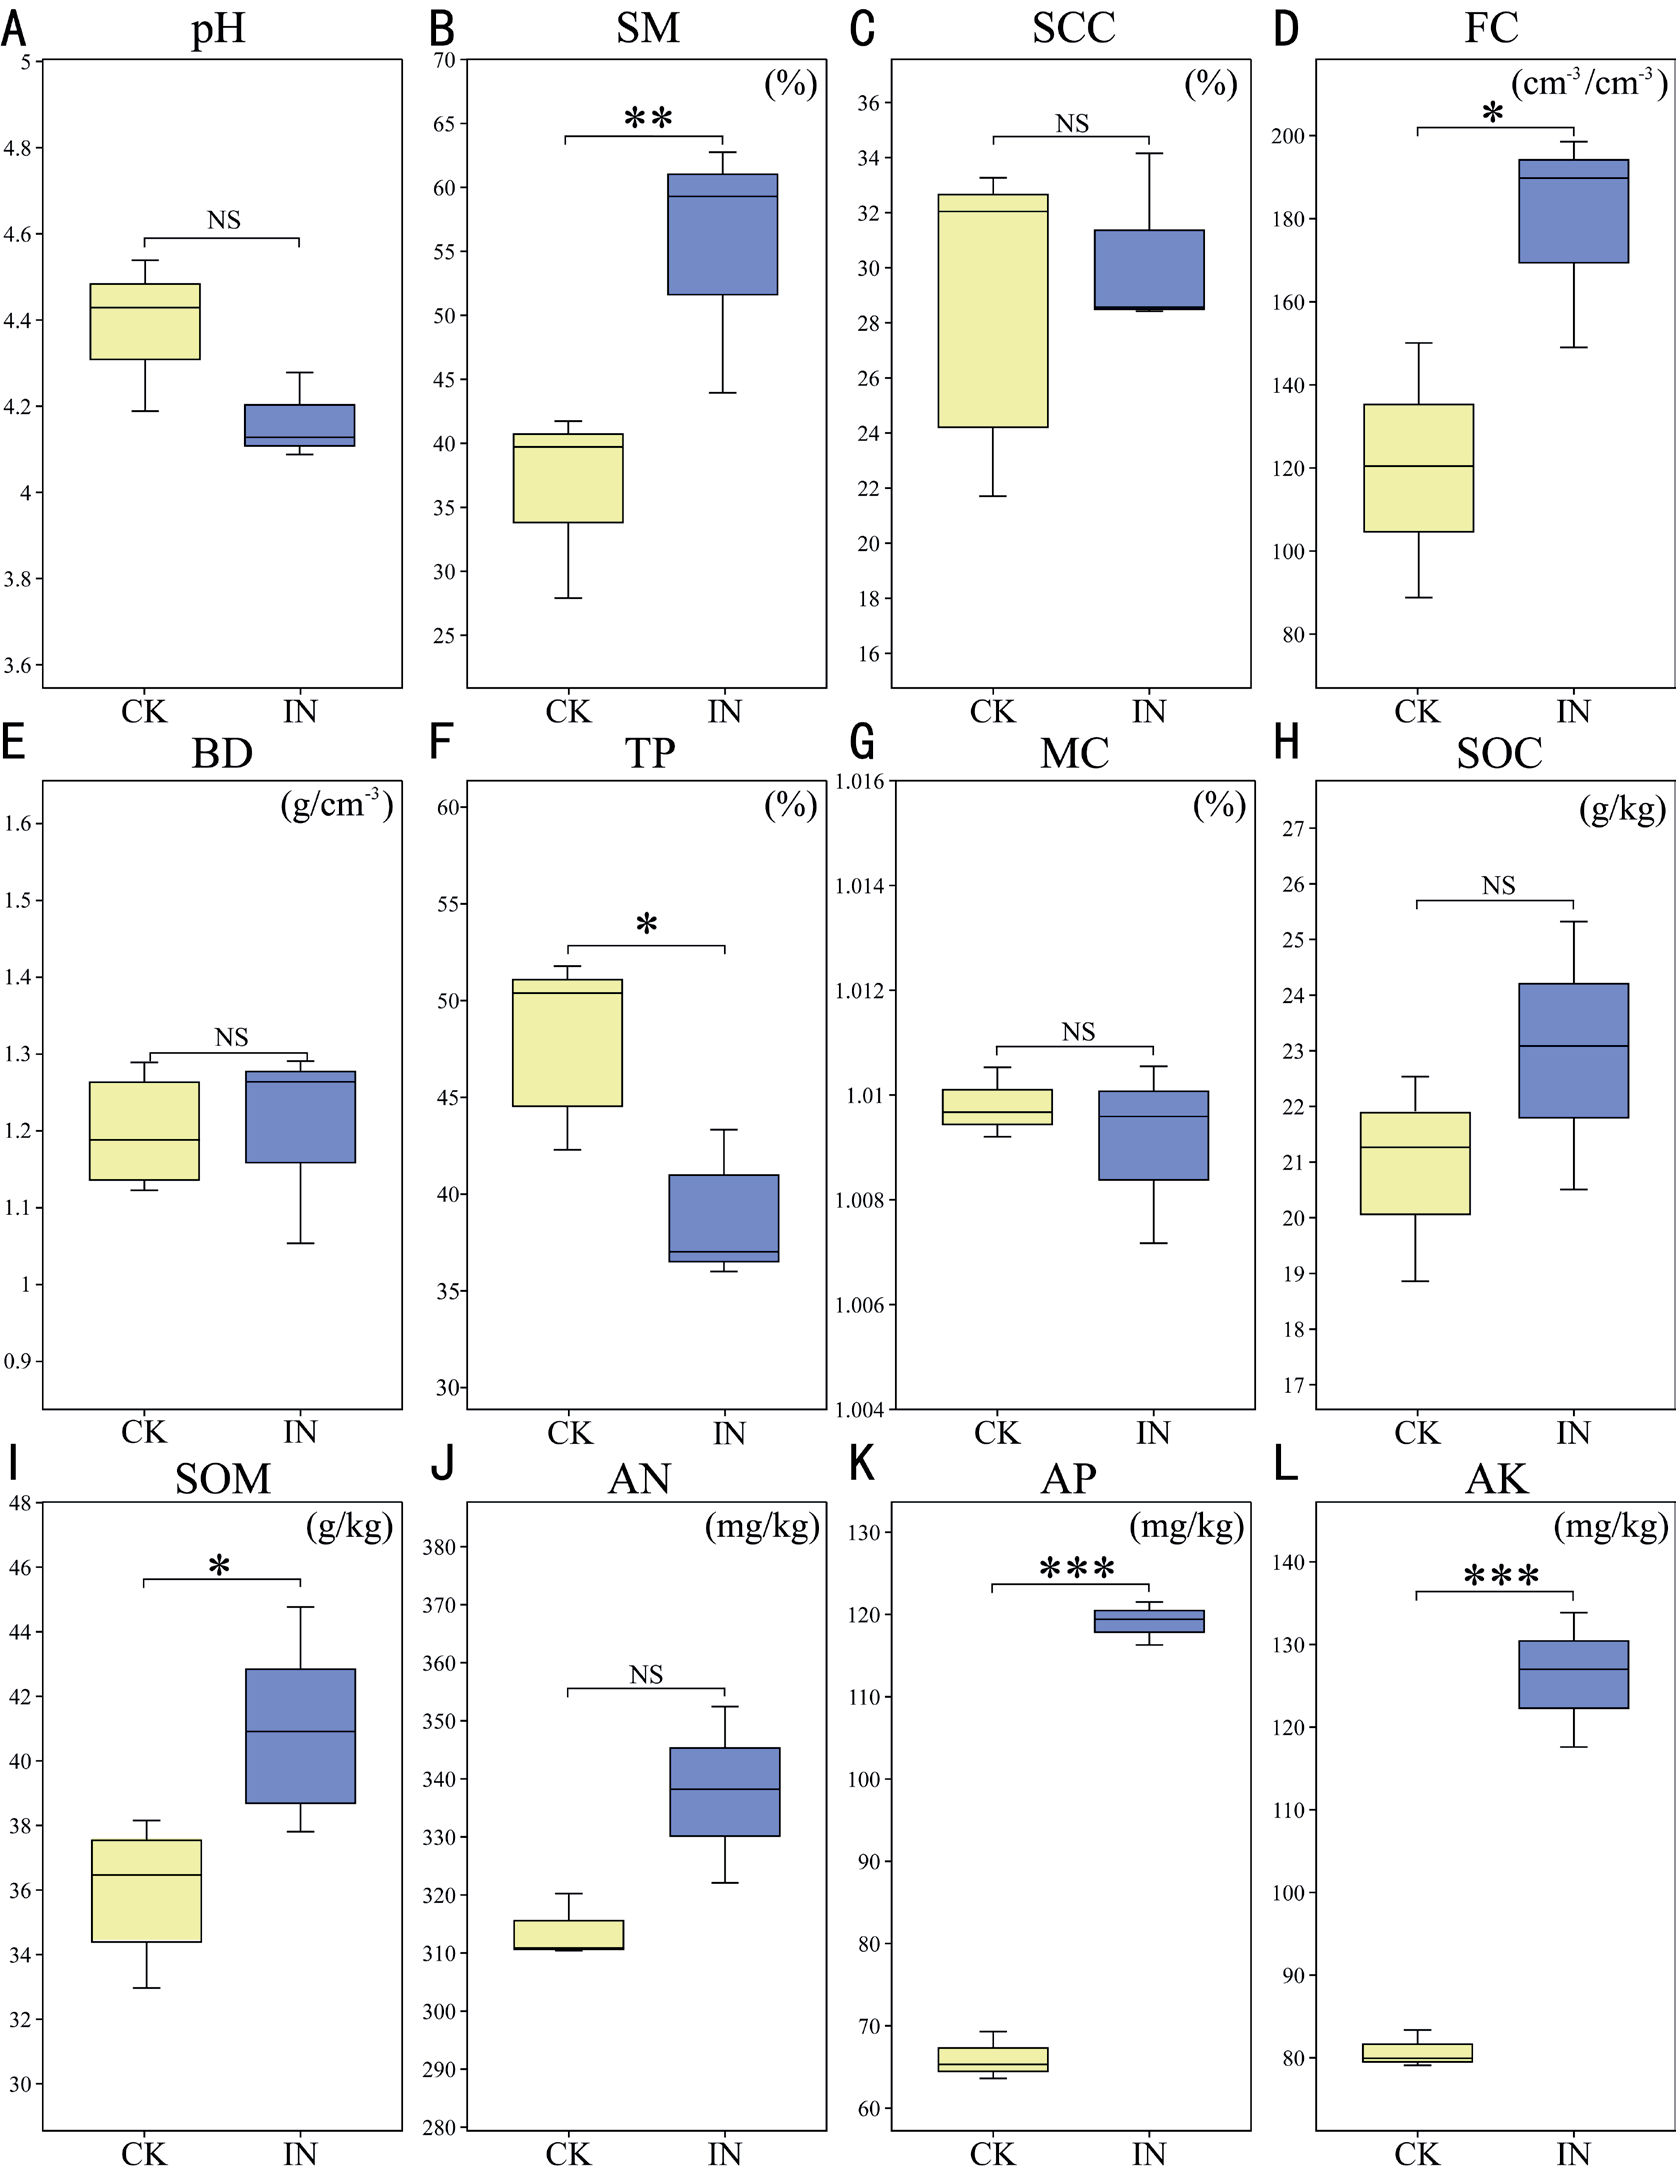
The results showed that, under the intercropping treatment, the soil saturated water content (SM) and field water-holding capacity (FC) increased significantly (p<0.05) by 49.07% and 48.77%, respectively. However, the changes in soil capillary water content (SCC) and moisture content (MC) were not statistically significant (p>0.05). Moreover, after intercropping, the total porosity (TP) of the soil significantly decreased by 20.46% (p<0.05) (Fig. 1).
Soil physicochemical properties serve as crucial indicators for assessing soil quality and conditions. The results indicated that the intercropping of bamboo fungus significantly influenced the nutrients contents in the soil (Fig. 1). After the intercropping treatment (IN), the pH value of the surface soil (0-20 cm) slightly increased compared to the control group (CK), with a pH of 4.53, indicating slightly acidic soil. Soil bulk density (BD) showed no significant change. While the organic carbon (SOC) and alkaline nitrogen (AN) content showed an upward trend under the IN treatment, these changes did not reach statistical significance (p>0.05). In contrast, the content of organic matter (SOM), available phosphorus (AP), and available potassium (AK) significantly increased under the IN treatment (p<0.05), with respective increases of 22.5%, 80.21%, and 56.13%.
Effects of Intercropping on the Bacterial Community Structure in Tea Plant Soil
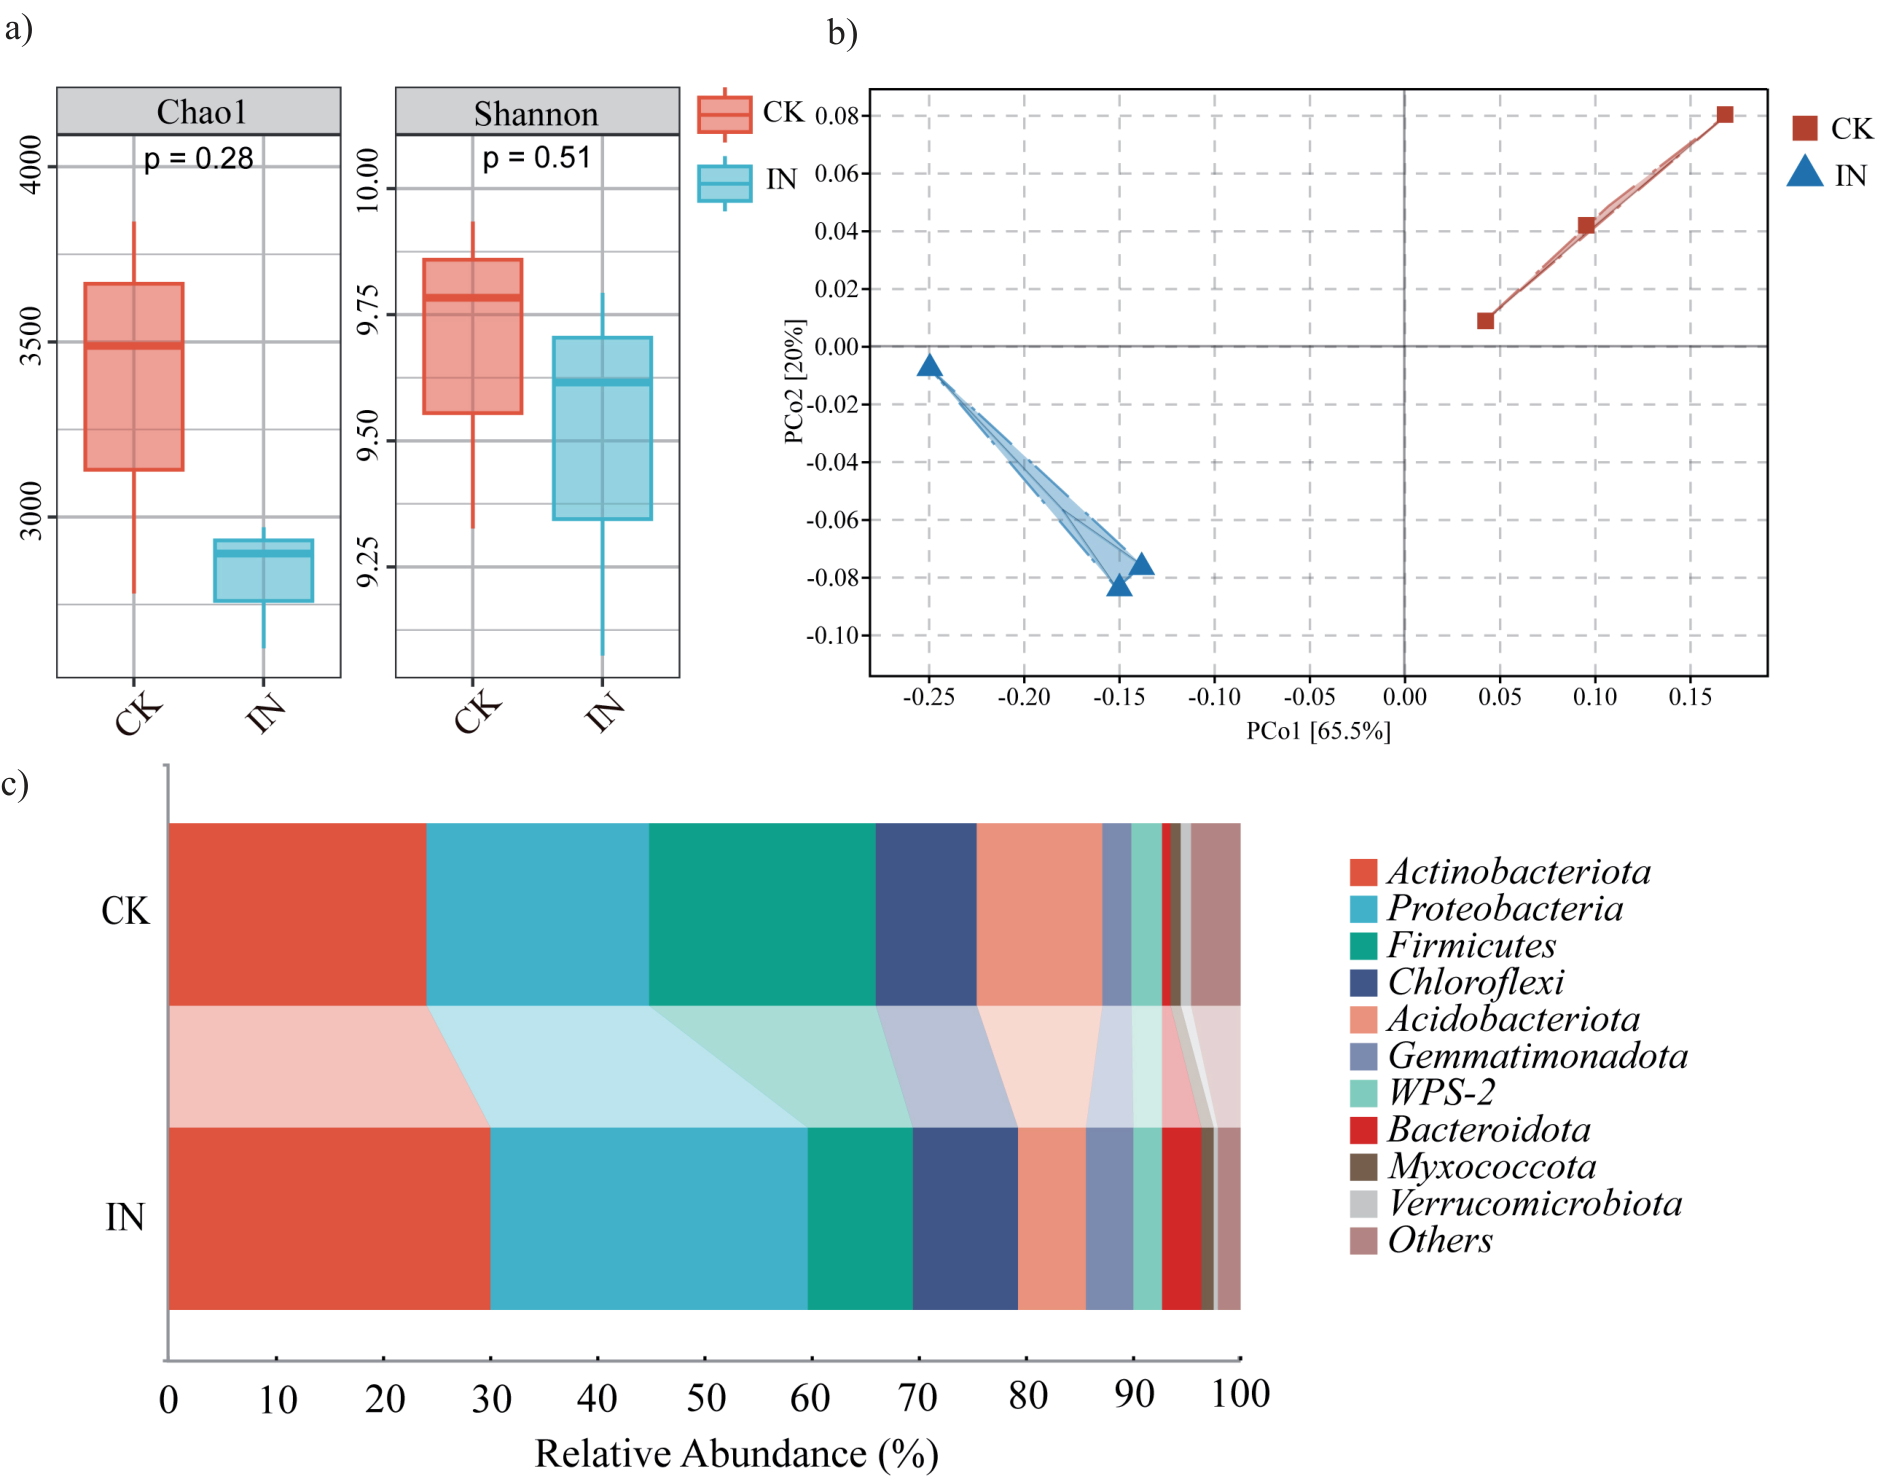
In this study, high-throughput sequencing was performed on soil samples collected from different treatments. The results showed that the Chao 1 index of bacteria in the bamboo fungus intercropping treatment (2797.83±172.64 OTU) decreased compared to the control treatment (3312.53±530.83 OTU), although this difference was not statistically significant (p>0.05). The Shannon index for the IN treatment was 9.434±0.359, which did not differ significantly from that of the CK treatment, which had a Shannon index of 9.630±0.304 (p>0.05) (Fig. 2a). Additionally, to assess the overall bacterial community differences across samples, a principal coordinate analysis (PCoA) based on the weighted Bray-Curtis distance matrix was conducted at the OTU level. This analysis revealed that PCoA1 and PCoA2 accounted for 86.5% of the variations in bacterial community structure among the different treatments. Notably, soil samples from the IN treatment clustered distinctly from those of the CK treatment, with clear intra-cluster grouping among bacterial communities, indicating that the IN treatment had a significant impact on the soil bacterial community (Fig. 2b).
Key Differential Bacterial Genera Selection
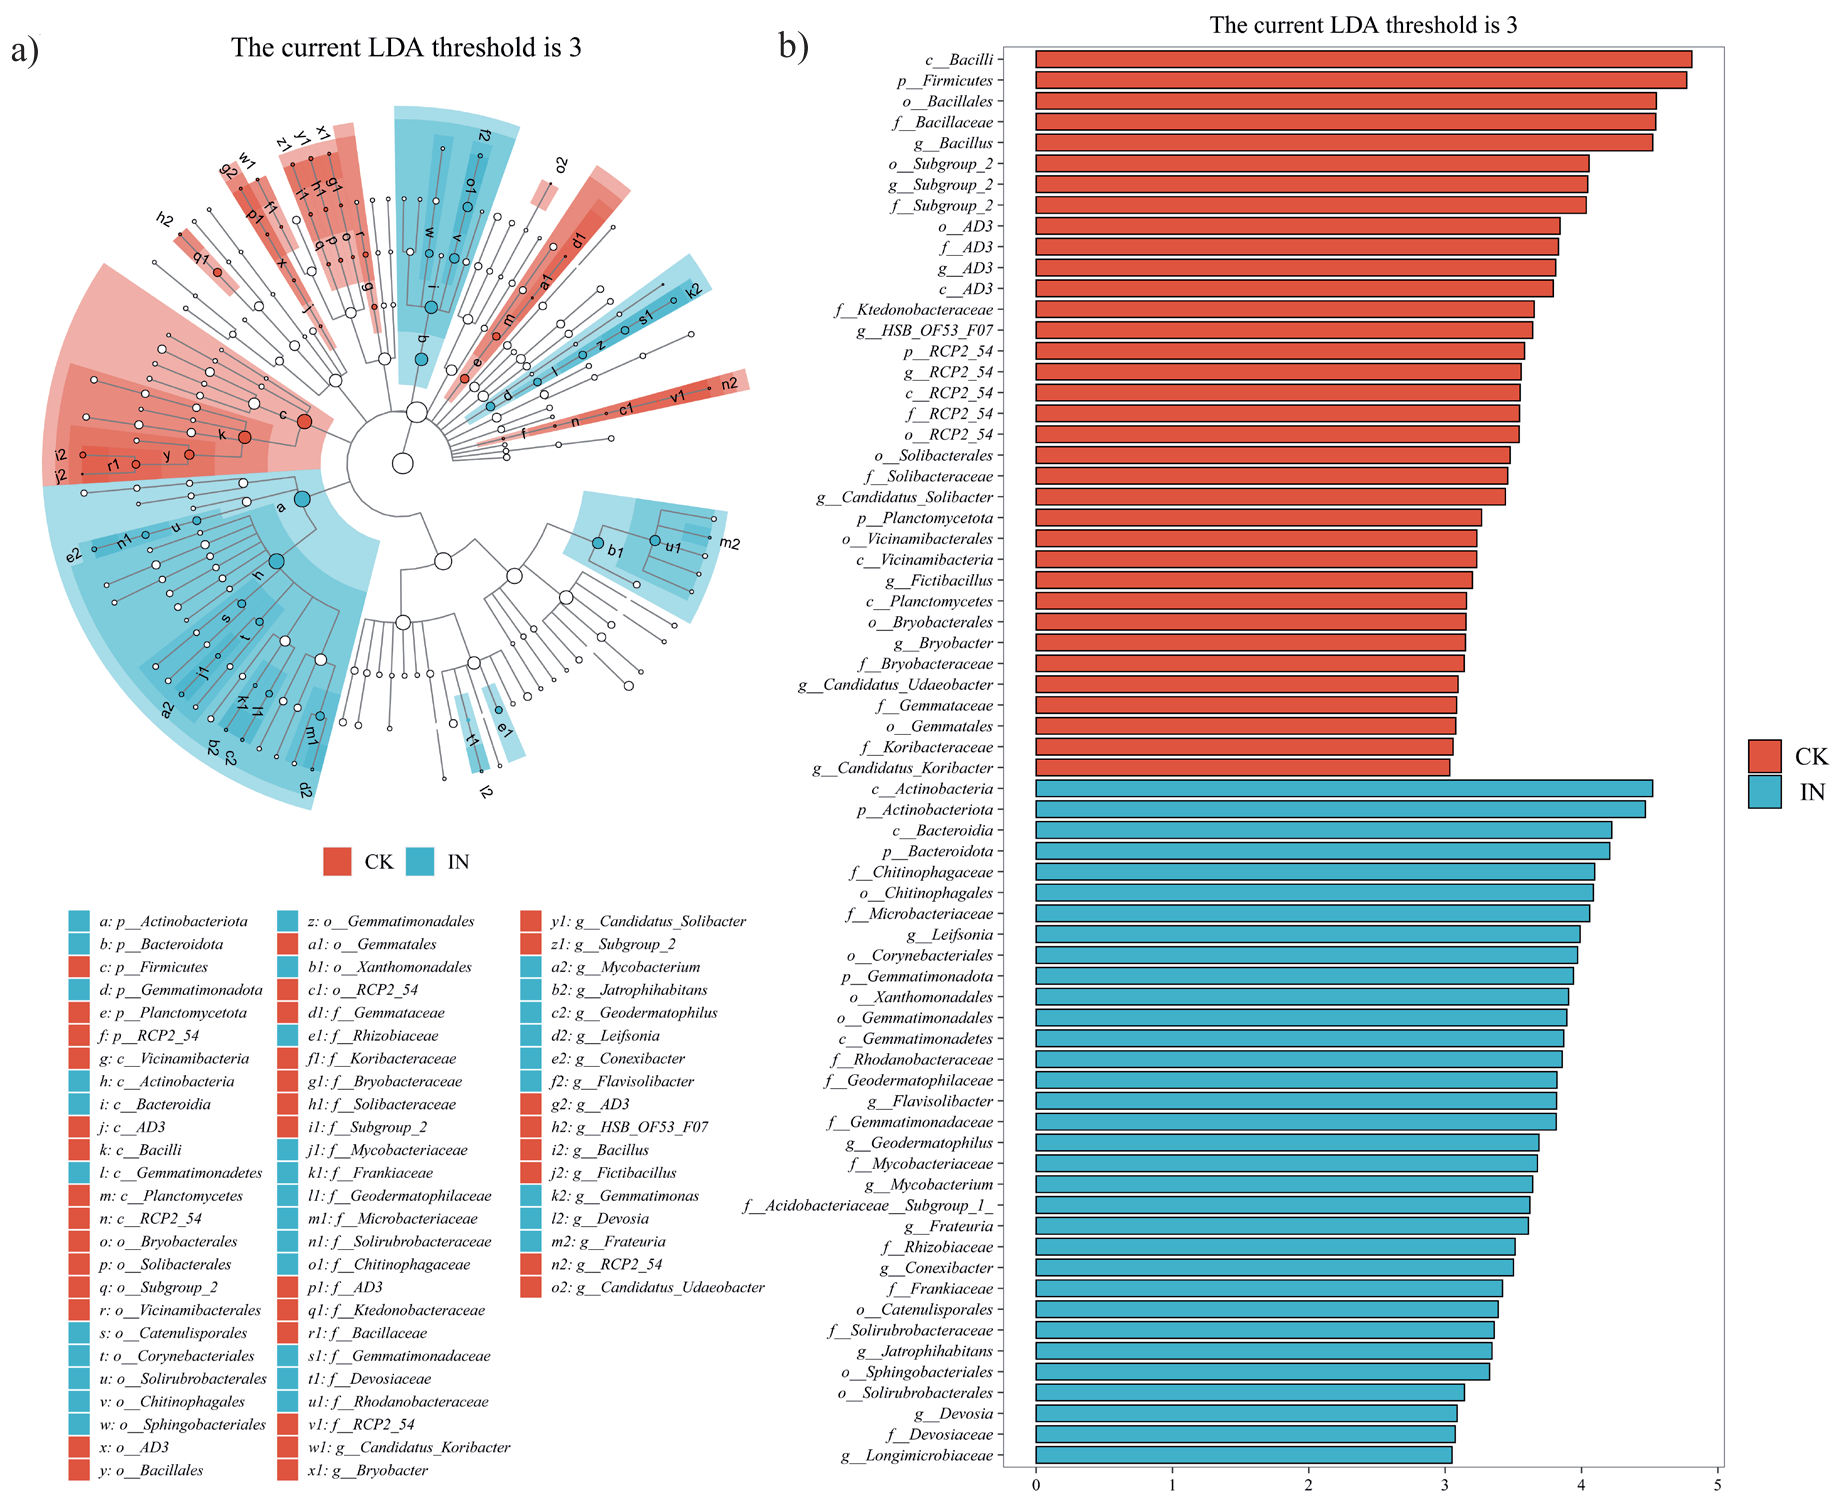
To further compare the significantly different bacterial species in tea plant soil, LEfSe analysis was performed to identify microbial groups at the phylum to genus level with distinct ecological niches (LDA>3) (Fig. 3). The results showed that six bacterial phyla, eight classes, fifteen orders, nineteen families, and nineteen genera exhibited significant differences across the various treatments. The identified nineteen genera were Candidatus_Koribacter, Bryobacter, Candidatus_Solibacter, Subgroup_2, Mycobacterium, Jatrophihabitans, Geodermatophilus, Leifsonia, Conexibacter, Flavisolibacter, AD3, HSB_OF53_F07, Bacillus, Fictibacillus, Longimicrobiaceae, Devosia, Frateuria, RCP2_54, and Candidatus_Udaeobacter. Among these, four important functional genera – Candidatus_Solibacter, Subgroup_2, Bryobacter, and Bacillus – were significantly enriched in the CK treatment. Notably, Gemmatimonadota, Devosia, Geodermatophilus, and Conexibacter were identified as core microbes that were recruited and enriched in the IN treatment, serving as valuable indicator species for differentiating between the treatments.
Fig. 1.
Soil moisture and soil physicochemical property indicators in tea gardens under intercropping (IN) and monoculture (CK) patterns. (A) pH, (B) Soil saturated water content, (C) Soil capillary water-holding capacity, (D) Field water-holding capacity, (E) Bulk density, (F) Total porosity, (G) Moisture content, (H) Soil organic carbon, (I) Soil organic matter, (J) Available nitrogen, (K) Available phosphorus, (L) Available potassium. The number of asterisks (*) indicates the significance level: p>0.05 = NS, p<0.05 = *, p<0.01 = **, p<0.001 = ***.
Effects of Intercropping on Soil Microbial Community Functions
The FAPROTAX database was used to annotate the ecological functions of soil microorganisms under different treatments, including nitrogen (N) and sulfur (S) cycles, as well as various substance degradation functions. Significant differences in bacterial functions were observed across treatments (p<0.05), indicating that the predictions for all operational taxonomic units (OTUs) were statistically significant. Analysis revealed that nitrogen cycling-related functions in bacteria underwent significant changes under intercropping. Five specific functions – denitrification, nitrite denitrification, nitrous oxide denitrification, nitrate denitrification, and nitrite respiration – demonstrated significant reductions compared to monoculture, with reductions of 70.89%, 83.31%, 84.86%, 79.63%, and 77.47%, respectively (p<0.05). Conversely, functions related to nitrogen respiration, nitrification, and nitrogen fixation significantly increased compared to monoculture, with increases of 12.32%, 31.91%, and 53.02%, respectively (p<0.05) (Fig. 4). In conclusion, compared to the CK treatment, the IN treatment showed a higher abundance of nitrogen cycling-related functions in the soil bacterial community after intercropping with bamboo fungus.
Effects of Intercropping on Soil Co-occurrence Networks Characteristics
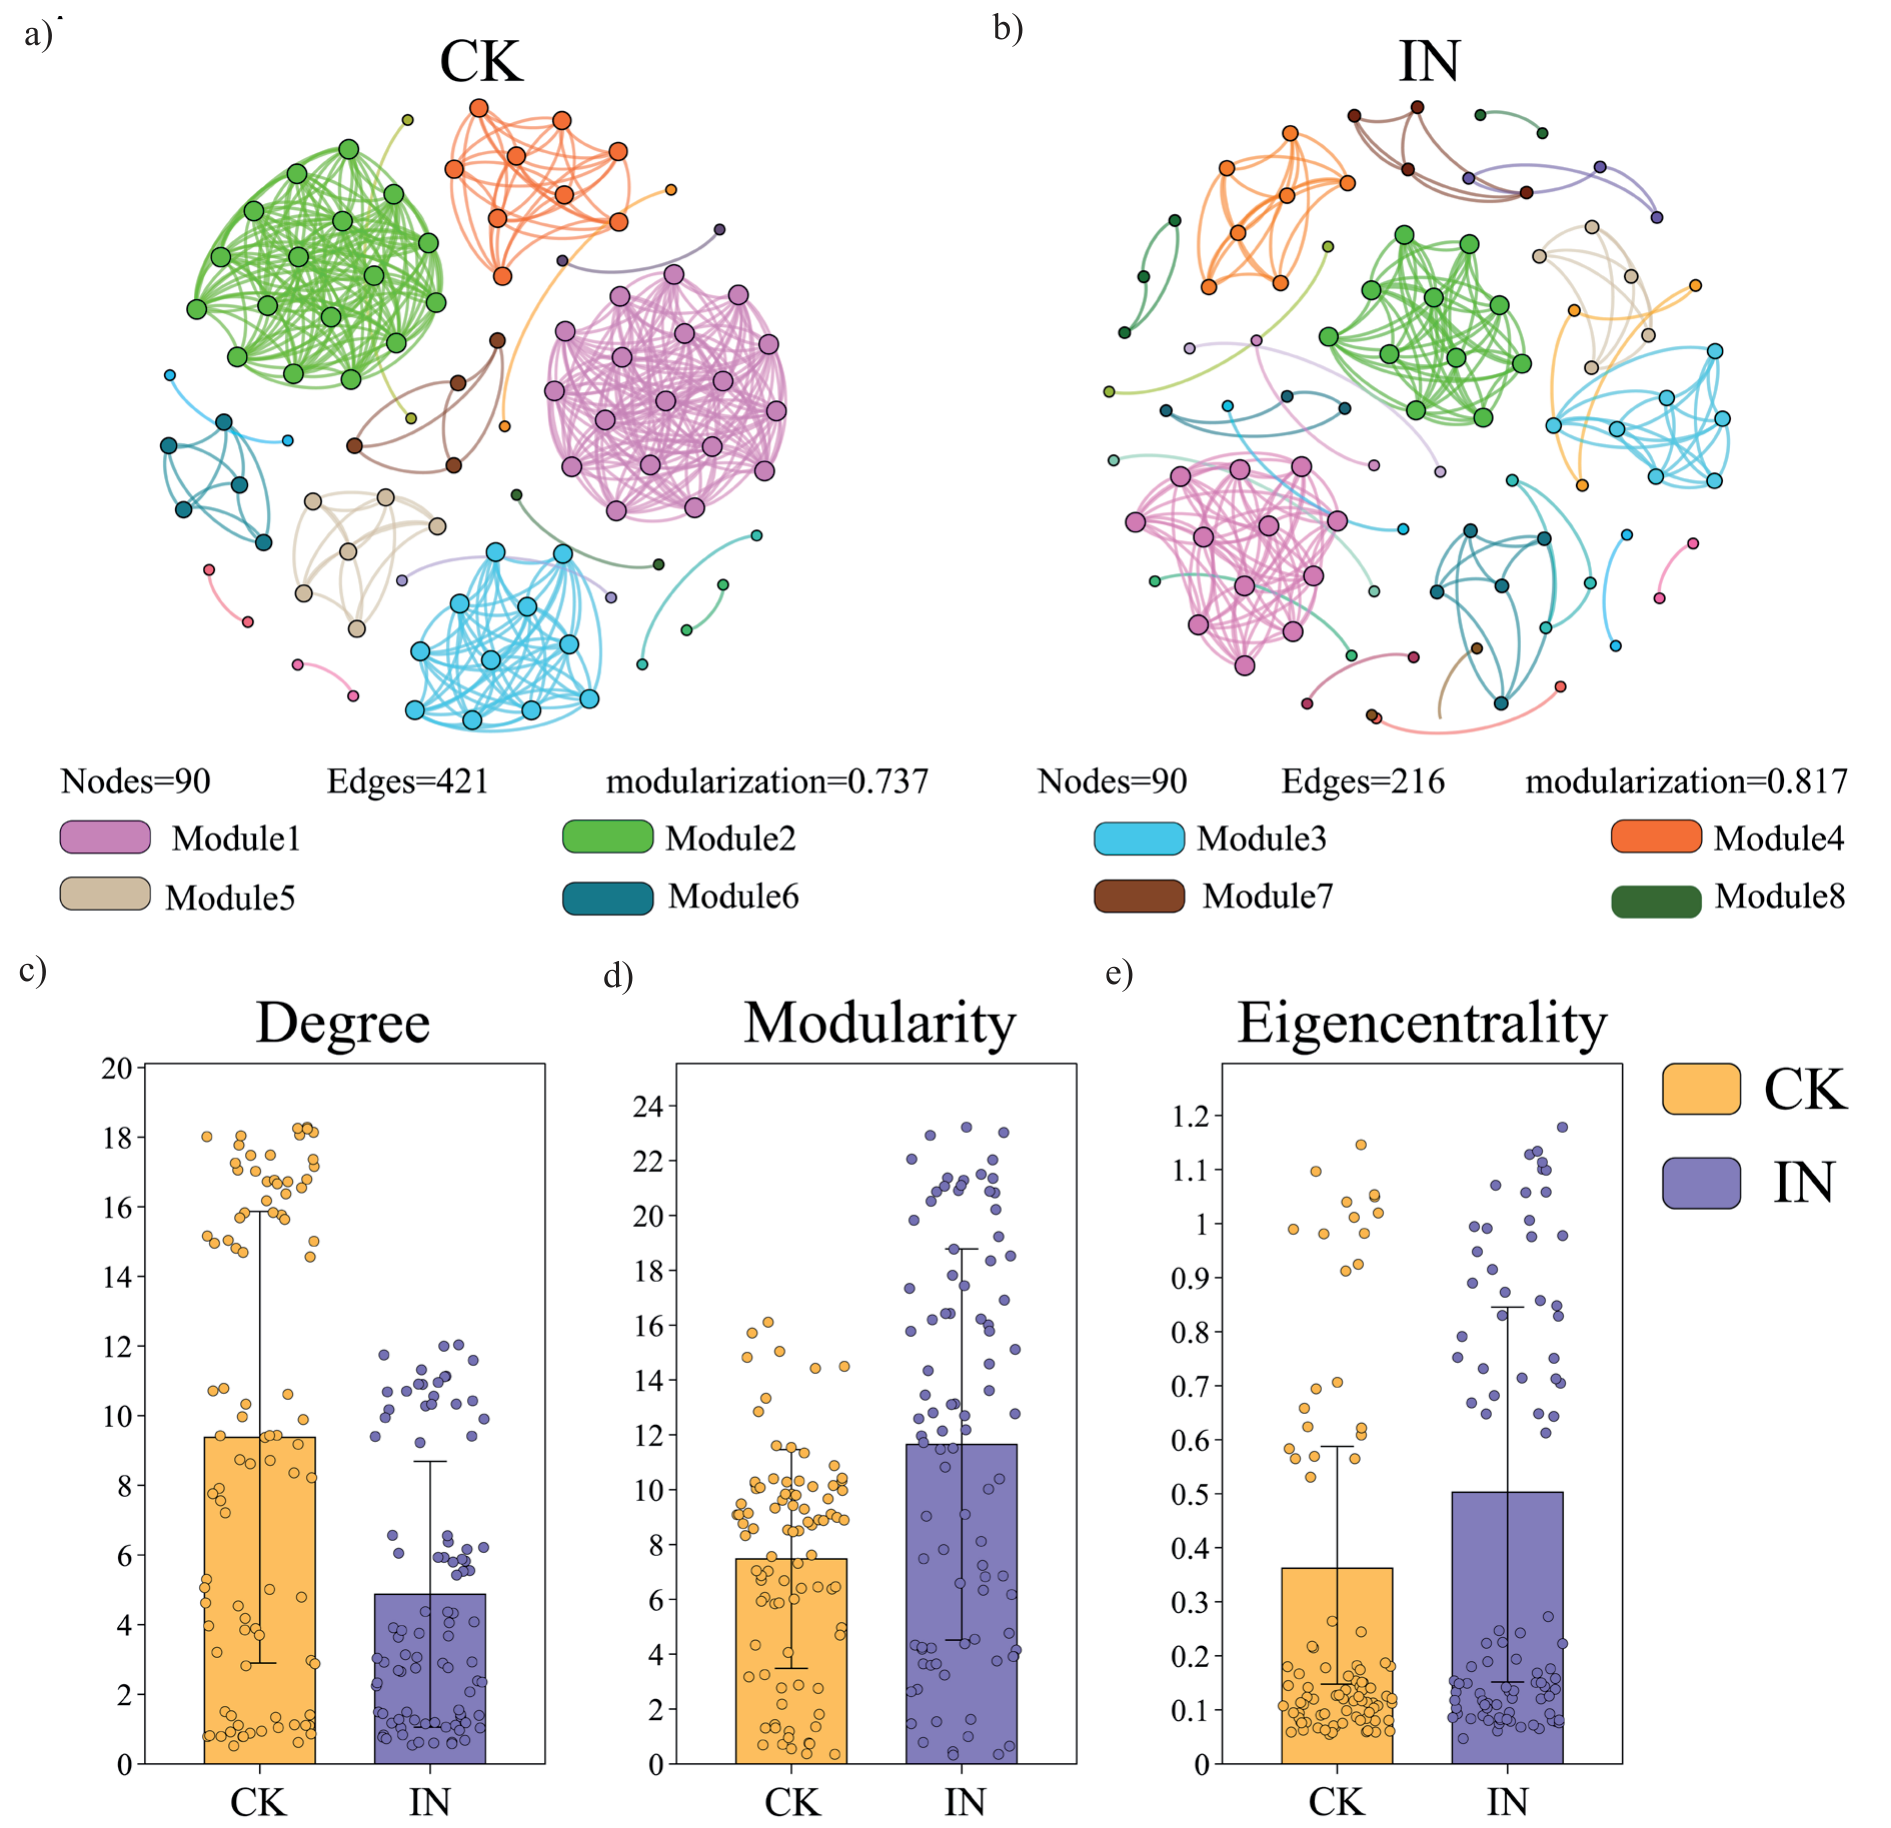
To explore the collinearity characteristics of soil microorganisms, co-occurrence networks analysis was performed to determine the symbiotic relationships within the microbial community under different planting systems. The analysis revealed (Fig. 5) that the average degree (9.356>4.8) and density (0.105>0.054) of the soil microbial symbiotic network were greater in monoculture tea plants than in intercropping with bamboo fungus. However, the modularity of the intercropping treatment (IN) was higher (0.737<0.817). Furthermore, the number of symbiotic network edges for dominant phyla such as Actinobacteriota, Proteobacteria, and Firmicutes significantly decreased in the intercropping treatment (216<421). Notably, after intercropping, both modularity and eigencentrality showed an increasing trend, indicating that key bacterial genera within the network had a stronger influence and greater centrality overall.
Interactions and Ecological Effects of Tea Plants and Bamboo Fungus Under Intercropping
Numerous studies have demonstrated that the advantages of intercropping are driven not only by niche differentiation and resource complementarity but also by root exudates and soil microorganisms [17, 18]. In particular, bamboo fungus and tea plants naturally occupy complementary ecological niches below ground [19], yet research on this aspect remains limited.
In this study, high-throughput sequencing was used to analyze the bacterial community structure in the rhizosphere of tea plants under different planting patterns. The results revealed significant differences in bacterial community structure between the intercropping and monoculture treatments (Fig. 1). Notably, after intercropping with bamboo fungus, the soil’s saturated water-holding capacity and field water-holding capacity increased significantly, while total porosity decreased. Additionally, the contents of organic carbon, alkaline nitrogen, organic matter, available phosphorus, and available potassium were all significantly higher in the intercropping system compared to monoculture [20]. Soil porosity plays a crucial role in preventing soil erosion and reducing drought stress on tea plants [21, 22]. The observed increase in moisture content alongside the decrease in soil porosity under intercropping suggests that this system helps reduce soil evaporation, thereby alleviating water stress to some extent [23]. This phenomenon may be due to the formation of a water retention network in the soil by the mycelium of bamboo fungus. The mycelium weaves through the soil, exhibiting strong water retention capacity that minimizes water infiltration and evaporation. Moreover, the fruiting bodies of bamboo fungus release trace amounts of water vapor during growth, which, combined with their occupation of pore spaces among soil particles, contributes to increased soil moisture content while reducing soil porosity [24, 25]. As key mediators in plant-soil interactions, microorganisms play a vital role in accelerating the decomposition of organic matter by enriching beneficial bacterial genera, thus regulating soil nutrient conditions.
Fig. 3.
Bacterial community composition LefSe analysis. a) Taxonomic cladogram (LDA > 3, comparing CK and IN groups). Different layers radiating outward from the center represent the branching levels of species classification. Each node corresponds to a specific classification at that level, while the color of the ribbons signifies different planting patterns. The letters on different nodes represent distinct bacterial species. b) LDA score plot for CK and IN treatments. A higher score indicates that a greater impact of species abundance on the intergroup differences.
Changes in Rhizosphere Microbial Diversity and Abundance of Specific Genera Under Intercropping
Diversity index analysis revealed no significant differences in the bacterial community diversity index of the rhizosphere under different intercropping treatments. Similar studies have noted that the Shannon index of bacterial, fungal, and archaeal communities in the rhizosphere of corn intercropped with various leguminous green manure crops did not show significant changes [26]. Comparable findings have been reported in intercropping systems involving wheat, potato/corn, and alfalfa/corn, where intercropping did not increase bacterial community diversity [27]. Some studies suggested that soil ecosystem functions primarily relied more on functional diversity than on taxonomic diversity [28, 29]. Additionally, research indicated that intercropping increased the abundance of key microbial groups in the soil [30]. In this study, the complexity of the symbiotic network in the intercropping treatment was lower than in monoculture. However, the increased modularity and eigencentrality values in the intercropping system suggest a more functional orientation and heightened centrality of individual nodes within the microbial symbiotic network. Thus, we speculate that the advantages of tea plant/bamboo fungus intercropping may not be directly related to changes in the taxonomic diversity of rhizosphere bacterial communities but rather influenced by specific functional bacterial genera within the rhizosphere.
Fig. 4.
Bacterial community functions predicted by FAPROTAX. Significance levels are as follows: * p<0.05, ** p<0.01, *** p<0.001.
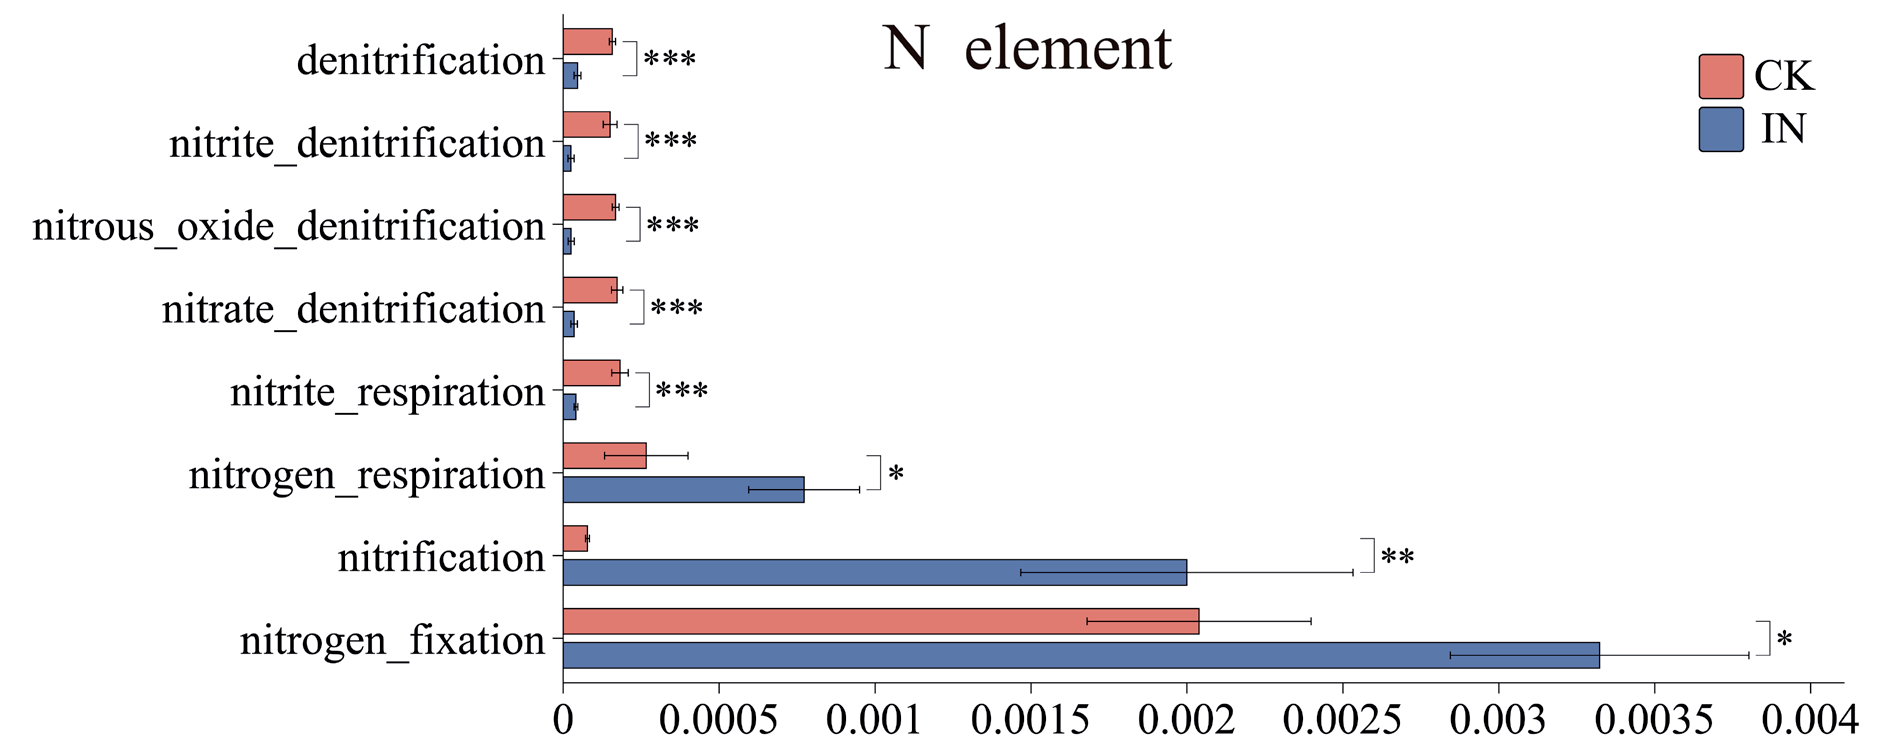
Further analysis of rhizosphere-specific functional bacterial communities revealed that the dominant bacterial phyla in the tea plant/bamboo fungus intercropping system were Actinobacteriota and Gemmatimonadota [31]. Numerous studies have documented that these phyla contribute to essential functions such as pathogen suppression, plant immune activation, promotion of plant growth, degradation of complex organic matter, and enhancement of soil nutrient cycling. Under intercropping conditions, Gemmatimonas, Devosia, Geodermatophilus, and Conexibacter were enriched at both the phylum and genus levels. These genera are commonly recognized as plant growth-promoting or biocontrol bacteria, especially with important roles in soil nitrogen cycling [32-35]. Functional predictions indicated that nitrification and nitrogen fixation functions were significantly enhanced, while nitrite denitrification, denitrification, and nitrate respiration functions were significantly reduced. This suggests that intercropping stimulated the activity of ammonia-oxidizing bacteria in the soil of tea plants, leading to increased conversion of urea to nitrate [36]. Notably, both nitrite denitrification and nitrate respiration are integral parts of the denitrification process, which reduces nitrate and nitrite to nitrogen gas, resulting in nitrogen loss in the soil. Therefore, the increase in nitrogen-enriched functions (such as nitrogen fixation, nitrogen respiration, and nitrification) and the decrease in nitrogen-loss functions (such as denitrification, nitrate denitrification, and nitrite denitrification) indicate an increase in soil nitrogen levels within the tea gardens [37, 38].
Interestingly, we observed a significant increase in soil pH and organic matter content under intercropping. Previous studies suggested that the decrease in pH under continuous monoculture often resulted from the release of organic acids by tea plant roots, the loss of alkaline ions from the soil, and the tea plant’s tendency to absorb ammonium nitrogen through proton exchange [39]. In the intercropping system, the observed increase in soil pH may be attributed to the increased quantity and diversity of organic matter, such as plant litter and root exudates, which enhance the metabolic activity and functionality of rhizosphere microorganisms. Additionally, the enrichment of functional microbial communities in the soil undoubtedly plays a significant role. Previous research has demonstrated that Conexibacter was a potentially advantageous species that facilitated ammonium nitrogen absorption via ammonium transport proteins (Amt) and engages in key processes within soil nitrogen cycling. Its enrichment may alter nitrogen forms and transformation processes in the soil, consequently influencing soil pH and promoting an increase in organic matter content [40]. In summary, the tea plant/bamboo fungus intercropping system enhances the enrichment of nitrogen-cycling-related bacterial genera such as Gemmatimonadota, Devosia, Geodermatophilus, and Conexibacter. This enrichment helps alleviate the negative feedback effects between plant and soil, accelerates nutrient cycling, and maintains overall soil health, thus promoting the growth of intercropped plants. Given the complexity of the relationship between plant root exudates and microorganisms, further research is needed to investigate the changes in root exudates under the tea plant/bamboo fungus intercropping system.
Fig. 5.
Comparison of bacterial co-occurrence network graphs in tea garden soils under different planting patterns. Co-occurrence networks of bacteria under monoculture (CK) treatment a) and intercropping (IN) treatment b). The size of the nodes is proportional to the number of their connections. The connections between nodes represent significant correlations (Spearman p<0.01, r>0.70), with different colors representing different modules in the network. Panels C, D, and E show the Degree c), Modularity d), and Eigencentrality e) of the symbiotic networks for CK and IN. Degree quantifies the total number of direct connections of a node. Modularity indicates the strength with which the network can be decomposed into discrete functional modules. Eigencentrality reflects the influence of a node within the core modules.
Conclusions
The tea plant/bamboo fungus intercropping system significantly enhanced the field water-holding capacity and available nutrient content of tea plant soil. By enriching nitrogen-cycling-related bacterial genera such as Gemmatimonadota, Devosia, Geodermatophilus, and Conexibacter, this intercropping system strengthened the nitrogen cycling functions of soil microbial communities, thereby enhancing nutrient cycling and facilitating the growth of tea plants. Therefore, tea plant/ bamboo fungus intercropping presents a promising approach for the sustainable development of tea gardens and offers robust support for the construction of green composite ecological tea plantation systems.

