

Introduction
Camellia sinensis (L.) O. Kuntze is a perennial cash crop cultivated in tropical and subtropical regions of over 50 countries worldwide [1]. In China, monoculture has traditionally been the prevalent cultivation model in tea plantations. However, the establishment of intercropped tea plantations has been increasingly adopted due to its documented advantages, particularly in maintaining long-term soil fertility compared to monoculture practices [2]. Intercropping systems rely less on external inputs such as fertilizers [3], which makes them particularly valuable for low-input or resource-limited agricultural models [4]. Intercropping involves cultivating one or more herbaceous/ shrub crops alongside trees in the same field, capitalizing plant growth characteristics and functional diversity to enhance resource utilization efficiency and benefit all crops involved [5].
Diversified agroforestry systems, including intercropping, are widely adopted globally due to the economic benefits derived from multiple crops [6]. Among various intercropping strategies, fungi-plant intercropping has gained recent attention and demonstrated positive effects on soil microbial communities and soil properties [7, 8]. For instance, Song et al. [7] reported beneficial effects of peach-Morchella intercropping on soil properties and fungal communities. Similarly, Chen et al. found that pear-Pleurotus ostreatus intercropping resulted in changes in soil microbial community structure, improved soil fertility, and enhanced fruit yield and quality [8]. In tea gardens, Ma et al. [9] found that tea-P. ostreatus intercropping significantly increased soil fungal diversity. Han et al. [10] conducted research on tea-Stropharia rugosoannulata intercropping, which led to significant improvement in soil organic matter content, total nitrogen, and available nitrogen content, reduced soil acidification and bulk density, and consequently improved soil structure. Intercropping tea plants with other fungal species, such as Oudemansiella radicata, also resulted in notable increases in soil available nitrogen, phosphorus, potassium content, and tea polysaccharide content [11]. Furthermore, fungal intercropping has been shown to enhance the abundance of bacteria and actinomycetes in the soil compared to monoculture tea gardens [12]. However, while numerous studies have highlighted the effects of fungi-plant intercropping on soil physicochemical properties, fungal communities, and crop quality and yield, the specific impacts on soil bacterial communities due to fungal intercropping have often been overlooked.
Bacteria, being a ubiquitous and essential component of the soil ecosystem, play a pivotal role in optimizing nutrient cycling, organic matter decomposition, and primary productivity of plants by promoting the diversity of soil bacterial communities [13, 14]. Previous studies had shown that the composition and diversity of soil bacterial communities were influenced by various factors, including plant species composition, soil type, and agricultural management practices [15, 16]. Understanding the role of soil bacterial communities, especially in agricultural ecosystems, and highlighting their ecosystem services and benefits is of utmost importance [17]. However, previous research on this topic has mainly focused on the effects of intercropping edible mushrooms on soil properties, tea yield, and soil fungi. Unfortunately, there is a relative scarcity of research regarding the composition and diversity of soil bacterial communities in tea plantations with intercropped fungi. Consequently, further investigations in this area are warranted.
Dictyophora indusiata (Vent.) Fisch., commonly known as bamboo mushroom, is an edible medicinal fungus belonging to the order Phallales and phylum Basidiomycota. As a saprophytic fungus, it thrives on decaying woody tree trunks or fertile soil in tropical regions of Africa, Asia, Australia, and the Americas [18], with low environmental requirements and easy cultivation. Additionally, its short growth cycle and straightforward sterilization methods make it a cost-effective and viable intercropping option with tea plants [19]. Surprisingly, no studies have explored the specific impact of bamboo mushroom intercropping with tea plants on the soil environment in tea plantations. Therefore, additional research is necessary to address this knowledge gap. Thus, this study focused on investigating the impact of intercropping D. Indusiata with tea trees on the structure and function of soil bacterial communities. To achieve this, 16S rRNA sequencing of rhizosphere soil bacteria was conducted. Additionally, certain physicochemical and enzymatic indicators of the soil were measured to analyze the changes in the overall soil environment caused by bamboo mushroom-tea plant intercropping. The aim was to reveal the relationships between these physicochemical and enzymatic indicators and the bacterial community.
Experimental Methods
Experimental Site and Soil Sample Collection
The current study was conducted in a tea plantation located in Ting Village, Jianyang District, Nanping City, Fujian Province, China (27°23’N, 118°16’E). The tea plantation experiences a typical subtropical monsoon climate in southern China, with an average annual temperature of 19°C and annual rainfall exceeding 2000 millimeters. Dictyophora indusiata was planted in January 2022 on the tea plantation, which comprises both monoculture and intercropping systems, and the same agronomic management strategies were implemented for both.
On October 8, 2022, during the fall season characterized by sunny weather and temperatures ranging from 20–25°C, soil samples were obtained from the rhizosphere of tea trees in both monoculture and intercropping systems with D. indusiata. The soil sampling procedure, employing a five-point sampling method mentioned by Xiong et al. [20], was utilized. From each system, two soil samples — marked as CK and Z — were gathered, and each sample had three replicates. The sampled tea trees were situated at analogous altitudes, slope positions, and aspects. The top layer of soil was meticulously excavated to enable sample collection from a depth spanning 5–20 centimeters beneath the tea tree roots. After collection, soil samples were promptly transported to the laboratory in an icebox. Each soil sample was divided into two portions: one was air-dried and ground using a 100-mesh sieve, while the other part was stored at -80°C in a freezer for DNA extraction. The samples were then sent to Shanghai Paiseno Biotechnology Co., Ltd. for DNA extraction, amplification, and high-throughput sequencing, aiming to determine the diversity and composition of soil bacteria.
Determination of Soil Physical and Chemical Indicators and Enzyme Activity Indicators
The soil pH value was determined using the water immersion extraction method with a soil-to-water ratio of 2.5:1. The field capacity of the soil was determined using the ring knife method. Soil organic carbon (SOC) was determined through the potassium dichromate oxidation method. The content of available nitrogen (SAN) was assessed using the alkaline hydrolysis diffusion method, while available phosphorus (SAP) content was determined using the molybdenum antimony anti-colorimetric method. The content of available potassium (SAK) was determined using the flame atomic absorption spectrophotometry method. These methods followed the guidelines established by Murphy and Riley [21], Knudsen et al. [22], and Dorich and Nelson [23].
Catalase activity in soil samples (S.CAT) was determined using a spectrophotometric method [24]. Soil dehydrogenase activity (S.DHA) was determined with triphenyltetrazolium chloride and iodonitrotetrazolium chloride [25]. Soil urease activity (S.UE) was measured using colorimetric determination of ammonium [26, 27]. Phosphatase activity (ACP) was determined using the p-nitrophenyl phosphate method [28].
DNA Extraction, PCR Amplification, and Sequencing
Genomic DNA was extracted from 0.5 g soil samples using the Soil DNA Isolation Kit (Omega Bio-tek, USA) following the manufacturer’s instructions. To assess the quality and concentration of the extracted DNA, three independent DNA extracts from each sample were combined, and their absorbance values were measured at 260 nm and 280 nm using a fluorescence spectrophotometer (Quantifluor-ST fluorometer, Promega, E6090; Quant-iT PicoGreen dsDNA Assay Kit, Invitrogen, P7589). Additionally, DNA quality was evaluated through 1% agarose gel electrophoresis. The DNA solution concentration was adjusted accordingly and stored at 4°C, while the storage solution was kept at -20°C.
The PCR amplification program consisted of an initial denaturation step at 95°C for 2 minutes, followed by 20 cycles of denaturation at 98°C for 10 seconds, annealing at 62°C for 30 seconds, extension at 68°C for 30 seconds, and a final extension at 68°C for 10 minutes. The amplification products of the bacterial 16S rRNA gene were visualized on a 2% agarose gel and purified using the AxyPrep DNA Gel Extraction Kit (Axygen Biosciences, Union City, California, USA). To determine the DNA concentration, quantification was performed using QuantiFluor-ST (Promega, Madison, Wisconsin, USA) assay. The purified amplicons were pooled in equimolar amounts and subjected to paired-end sequencing (2×250) on the Illumina platform using standard protocols. The constructed sequencing library was prepared using Genedenovo on the Illumina HiSeq2500 PE250 platform (Personal Biotechnology Co., Ltd., Shanghai, China).
Data Analysis
Statistical analysis was performed using SPSS software to evaluate significant differences in soil physicochemical and enzyme activity indicators. High-throughput sequencing of soil bacterial 16S rDNA was carried out by Shanghai Personal Biotechnology Co., Ltd. Upon standardizing the soil microbial community data, analyses of α-diversity and Principal Coordinate Analysis (PCoA) were conducted employing the Bray–Curtis algorithm. The taxonomic composition analysis and rarefaction curve were performed using QIIME2 (version 2019.4). Boxplots of the Chao1 index, Observed species index, Simpson index, and Shannon index were generated using GraphPad Prism 8. Relative abundance plots at the phylum level were created using the ggplot2 package in R (version 4.3.1). Manhattan plots at the genus level were also generated using R (version 4.3.1). The Venn diagram of OTUs was constructed using the VennDiagram package in R. PCA clustering analysis was conducted using the Vegan package in R (version 4.3.1). Correlation heatmaps were generated using TBtools.
Results
Effects of Intercropping D. indusiata and Tea on Soil Physicochemical and Enzyme Activities
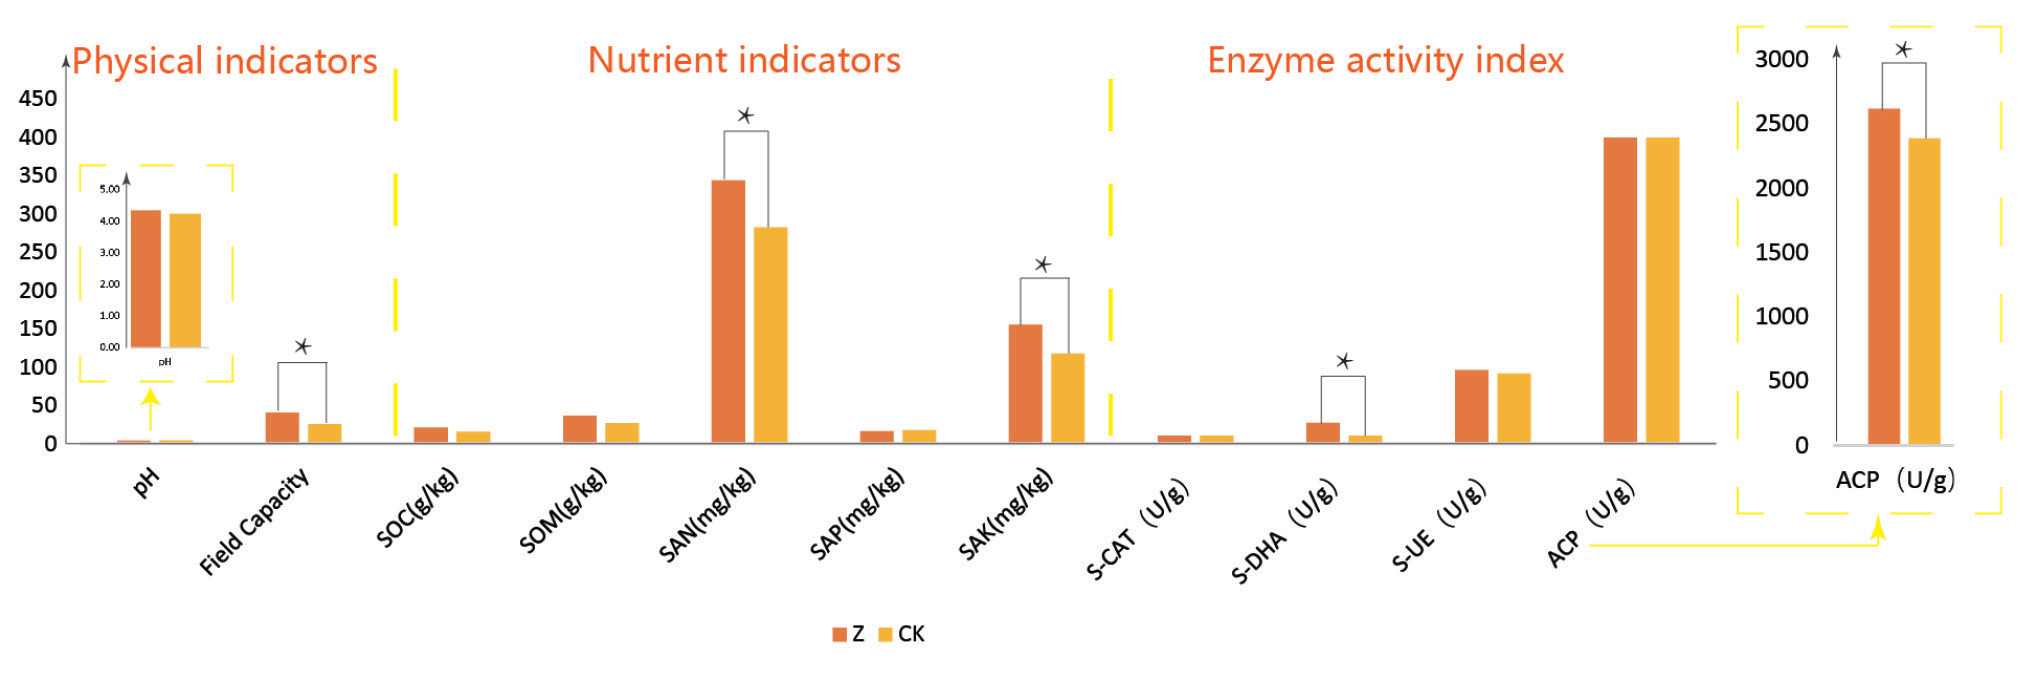
The results in Fig. 1 reveal that, in comparison to the monoculture soils, the intercropped soils did not show a significant change in pH. However, a significant increase was observed in the field capacity of the intercropped soils. Several nutrient indicators, including organic carbon, organic matter, available nitrogen, and available potassium content, displayed a noticeable improvement in the intercropped soils. Additionally, we observed varying degrees of increase in the four measured soil enzyme activities, with soil dehydrogenase (S-DHA) and soil acid phosphatase (ACP) showing the most significant increases. Overall, the intercropped bamboo mushroom-tea plant soils outperformed the monoculture soils in several physicochemical and enzymatic indicators.
Changes in Soil Microbial Community Diversity
α-Diversity Analysis
The soil bacterial community was assessed using high-throughput 16S rDNA amplicon sequencing. After filtering the raw sequencing data, high-quality CCS reads generated by the sequencing platform were retained. On average, there were 100,678 soil bacterial community sequences in single-cropping soil samples and 112,378 in the intercropping soil samples. The bacterial diversity curve (Fig. 2E) approached asymptotes, indicating that sufficient sequencing depth for most samples. The Chao1 index (Fig. 2A) and Observed species index (Fig. 2B) represented richness, while the Shannon index (Fig. 2D) and Simpson index (Fig. 2C) represented diversity. The figure showed that the bamboo mushroom-tea intercropping model exhibited higher richness and diversity of soil microbiota compared to single tea cropping, although the differences were not statistically significant. The coverage of soil bacterial diversity was > 0.99 for all samples, indicating that the sequencing depth accurately reflected the true bacterial composition in the soil samples.
β-Diversity Analysis
To explore the dissimilarities in bacterial community structure between the two treatments, we employed β diversity analysis, specifically using the Bray-Curtis distance algorithm and conducting principal coordinate analysis (PCoA). The PCoA results (Fig. 2E) revealed a distinct clustering of bacterial members based on the sampling regions. Notably, the bacterial communities in the two treatments exhibited discernible differences, with samples from each treatment group distributed on opposite sides of the x-axis. This finding indicated that the intercropping treatment had the capacity to modify the composition of the tea garden soil bacterial community.
Based on the Venn diagram (Fig. 2G), the soil bacterial community exhibited a total of 12,819 operational taxonomic units (OTUs). Among them, 7,770 OTUs were observed in the intercropping soil samples, while 6,891 OTUs were found in the single-cropping soil samples. Surprisingly, only 1,842 OTUs were shared between the two groups, constituting a mere 14.4% of the total OTUs. These findings suggest that the intercropping treatment has the potential to significantly alter the structure of the bacterial community and exert an influence on its diversity.
Changes in Soil Microbial Community Composition and Structure
The two types of soil commonly found in tea gardens exhibited a relatively high abundance of 13 bacterial phyla, including Proteobacteria, Acidobacteria, Chloroflexi, Actinobacteria, Gemmatimonadetes, Firmicutes, WPS-2, Verrucomicrobia, Patescibacteria, Planctomycetes, Nitrospirae, Bacteroidetes, and Rokubacteria. Intercropping D. indusiata and tea trees resulted in significant changes in the relative abundance of certain phyla. Specifically, the relative abundance of Proteobacteria, Gemmatimonadetes, Firmicutes, WPS-2, Patescibacteria, Nitrospirae, and Bacteroidetes significantly increased, while Acidobacteria and Rokubacteria decreased. The relative abundance of other phyla remained relatively stable. In the single cropping soil, nine bacterial phyla exhibited relative abundance higher than 0.01, while in the intercropping soil, 12 bacterial phyla exhibited relative abundance higher than 0.01. Patescibacteria, Nitrospirae, and Bacteroidetes showed increased abundance (> 0.01) in the intercropping soil. The pie chart (Fig. 3) clearly depicted a relatively homogeneous bacterial community structure in the single cropping group, with a significant proportion attributed to the dominant four phyla in the tea garden and the remaining 11% assigned to other less abundant phyla. Following the intercropping treatment, the relative abundance of some less abundant phyla significantly increased. Moreover, aside from the dominant four phyla, the remaining phyla enriched to 17.5%. Therefore, intercropping has induced alterations in the bacterial community structure, resulting in a substantial increase in bacterial community diversity.
Fig. 2.
(A) CHAO1 index, (B) Observed specifications index, (C) Simpson index, (D) Shannon index, (E) Rarefied fraction curves, (F) PCoA analysis of soil bacterial community, (G) Venn diagrams of core OTUs of soil bacteria in different planting modes.
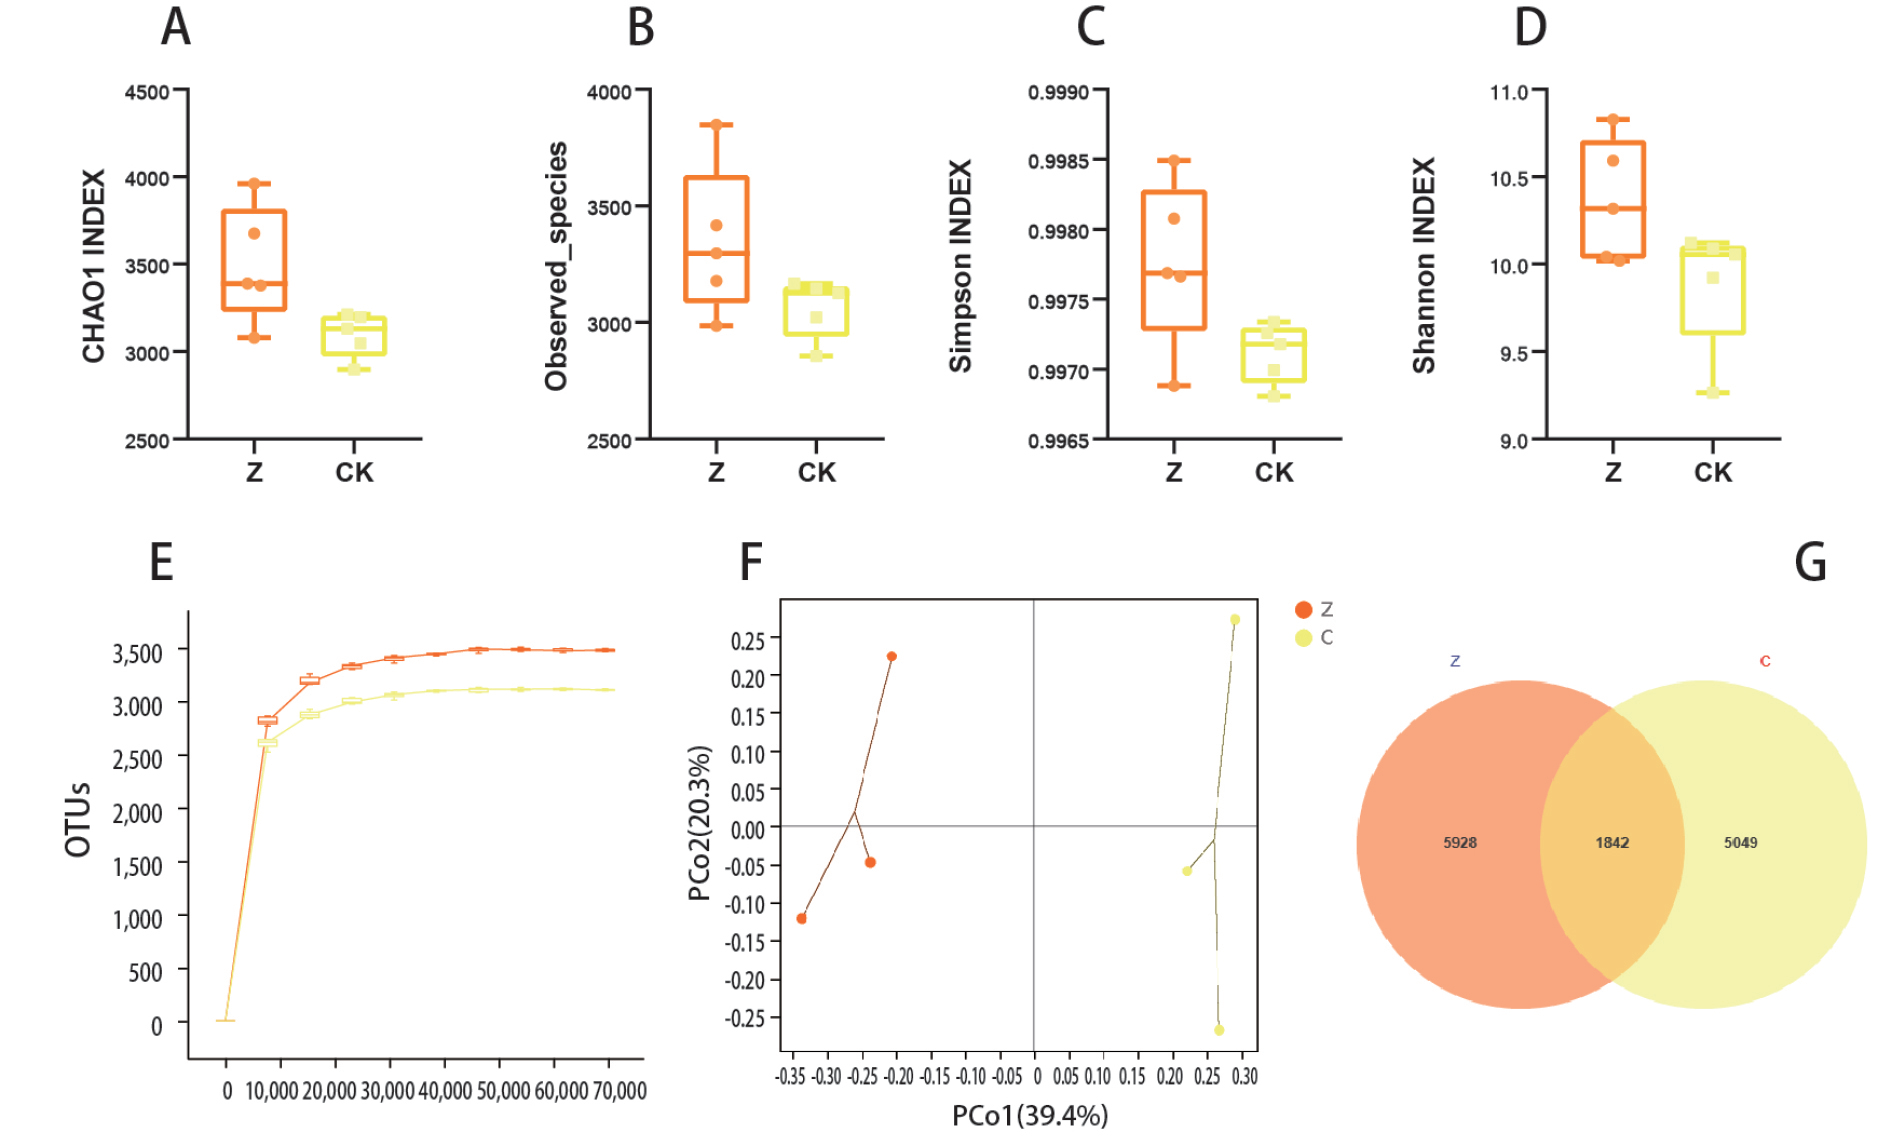
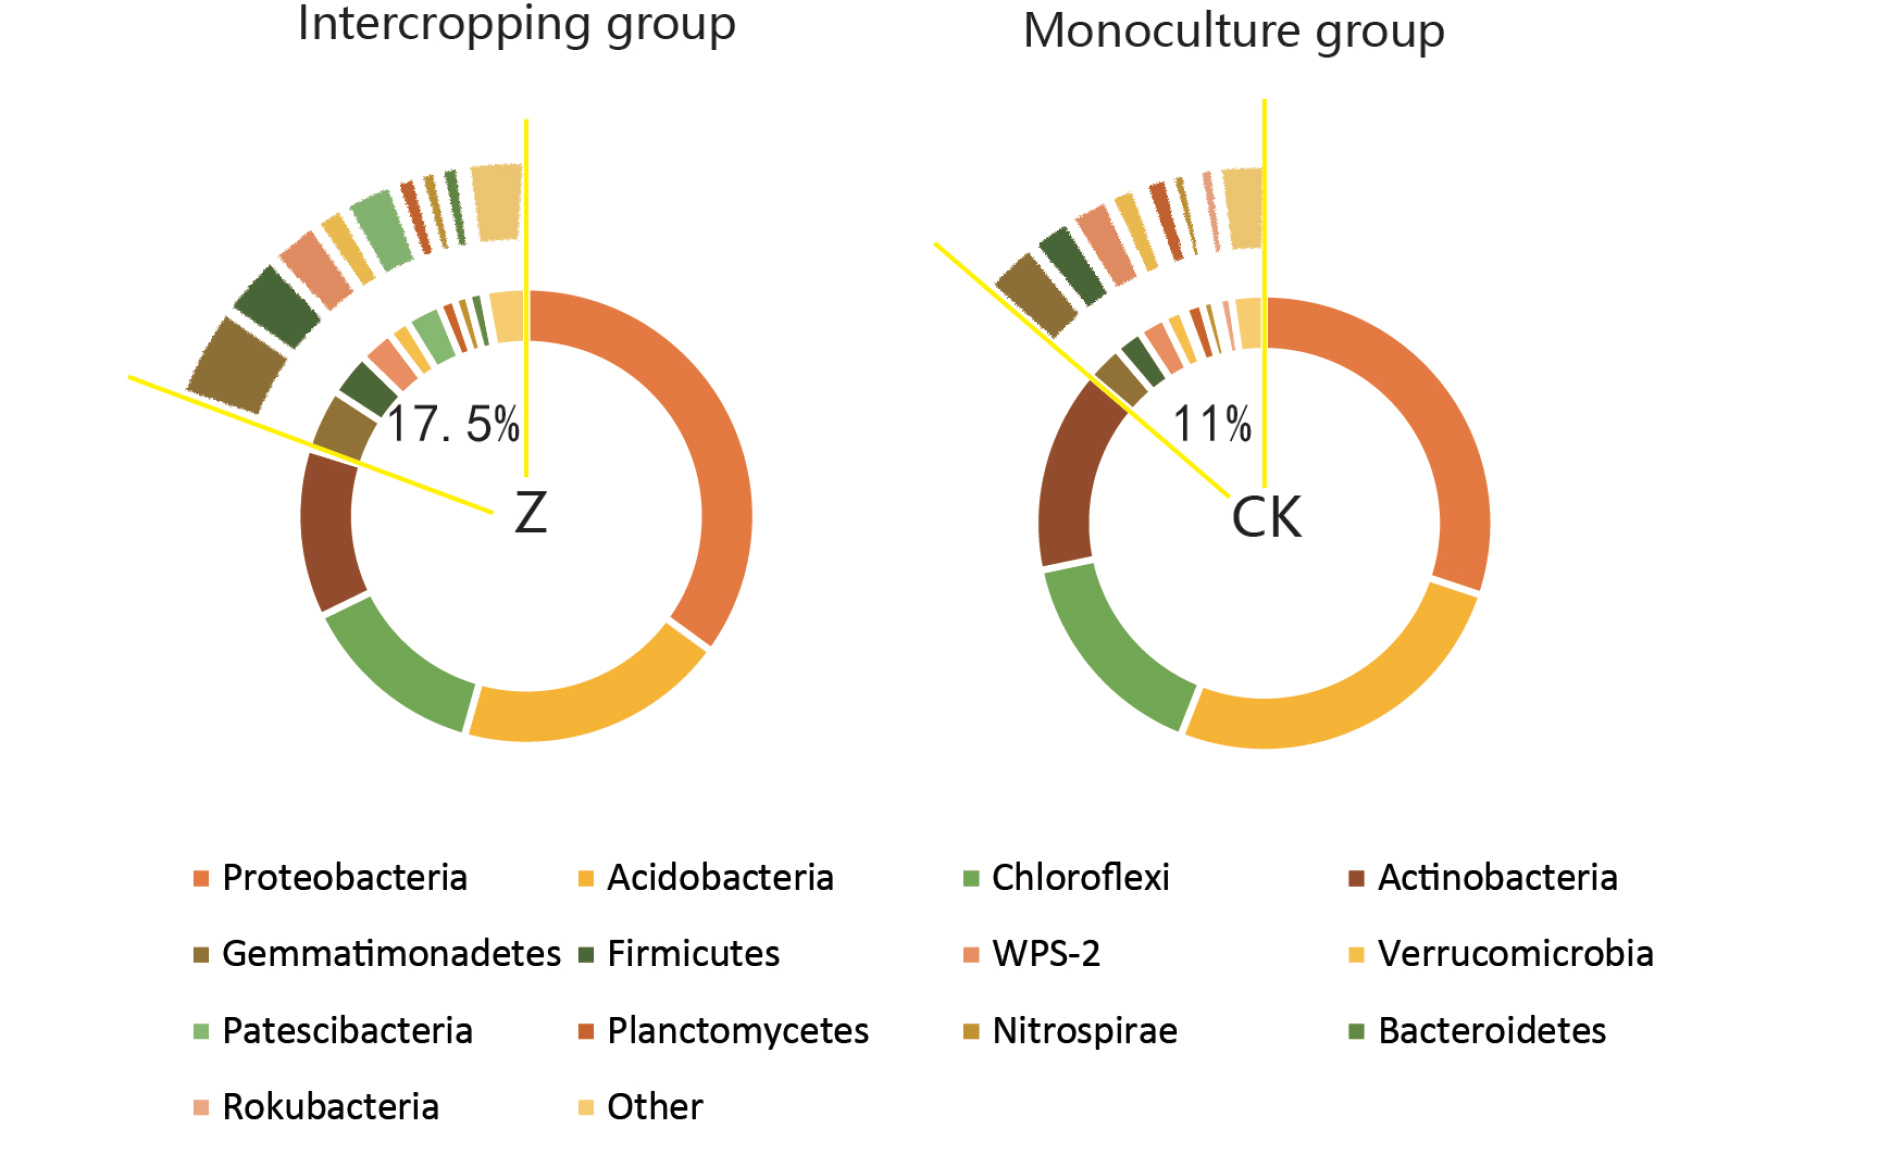
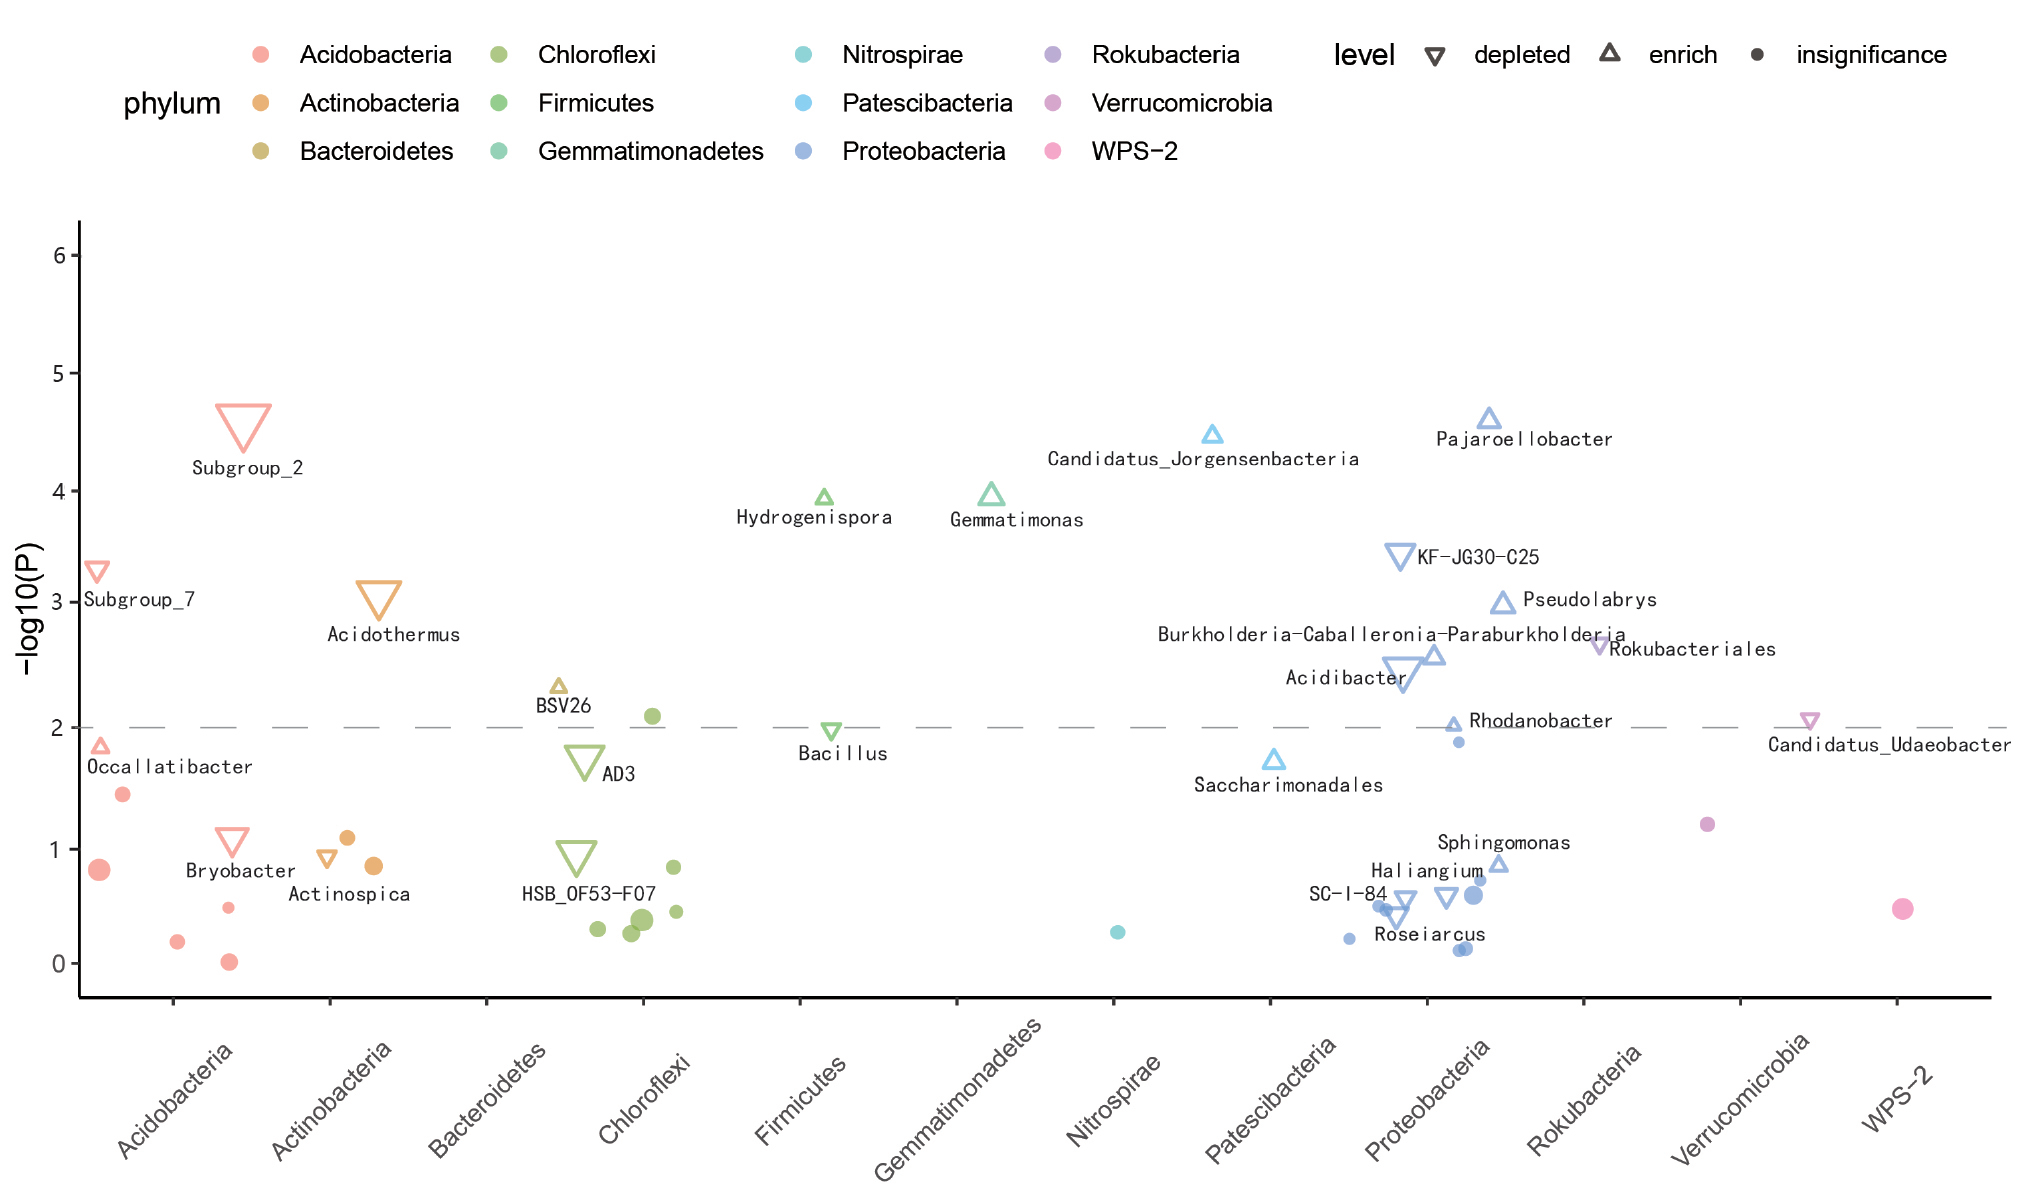
Fig. 4 presented a Manhattan plot based on our analysis of the genus level, focusing on the top 50 genera. In the intercropping soil, we observed significantly different genera among the three phyla, exhibiting a relative abundance increase of greater than 0.01. Notably, the plot highlighted that the significantly different genera are predominately concentrated in the four dominant phyla in tea gardens: Proteobacteria, Acidobacteria, Chloroflexi, and Actinobacteria. Specifically, compared to the single cropping group, the intercropping group showed upregulation of Candidatus_Jorgensenbacteria, Rhodanobacter, Saccharimonadales, Occallatibacter, Hydrogenispora, Gemmatimonas, Pseudolabrys, Burkholderia-Caballeronia-Paraburkholderia, Sphingomonas, Pajaroellobacter, and BSV26. Conversely, Haliangium, Bryobacter, Acidibacter, Acidothermus, Bacillus, Candidatus_Udaeobacter, Actinospica, and Rokubacteriales showed downregulation in the intercropping group. Among them, Acidothermus, Bryobacter, Acidibacter, Gemmatimonas, Pajaroellobacter, and Pseudolabrys exhibited more pronounced fold changes. In summary, these findings indicated that intercropping practices promoted the recruitment of specific bacteria, leading to alterations in the distribution and abundance of microbiota at both the phylum and genus levels.
Correlation Analysis
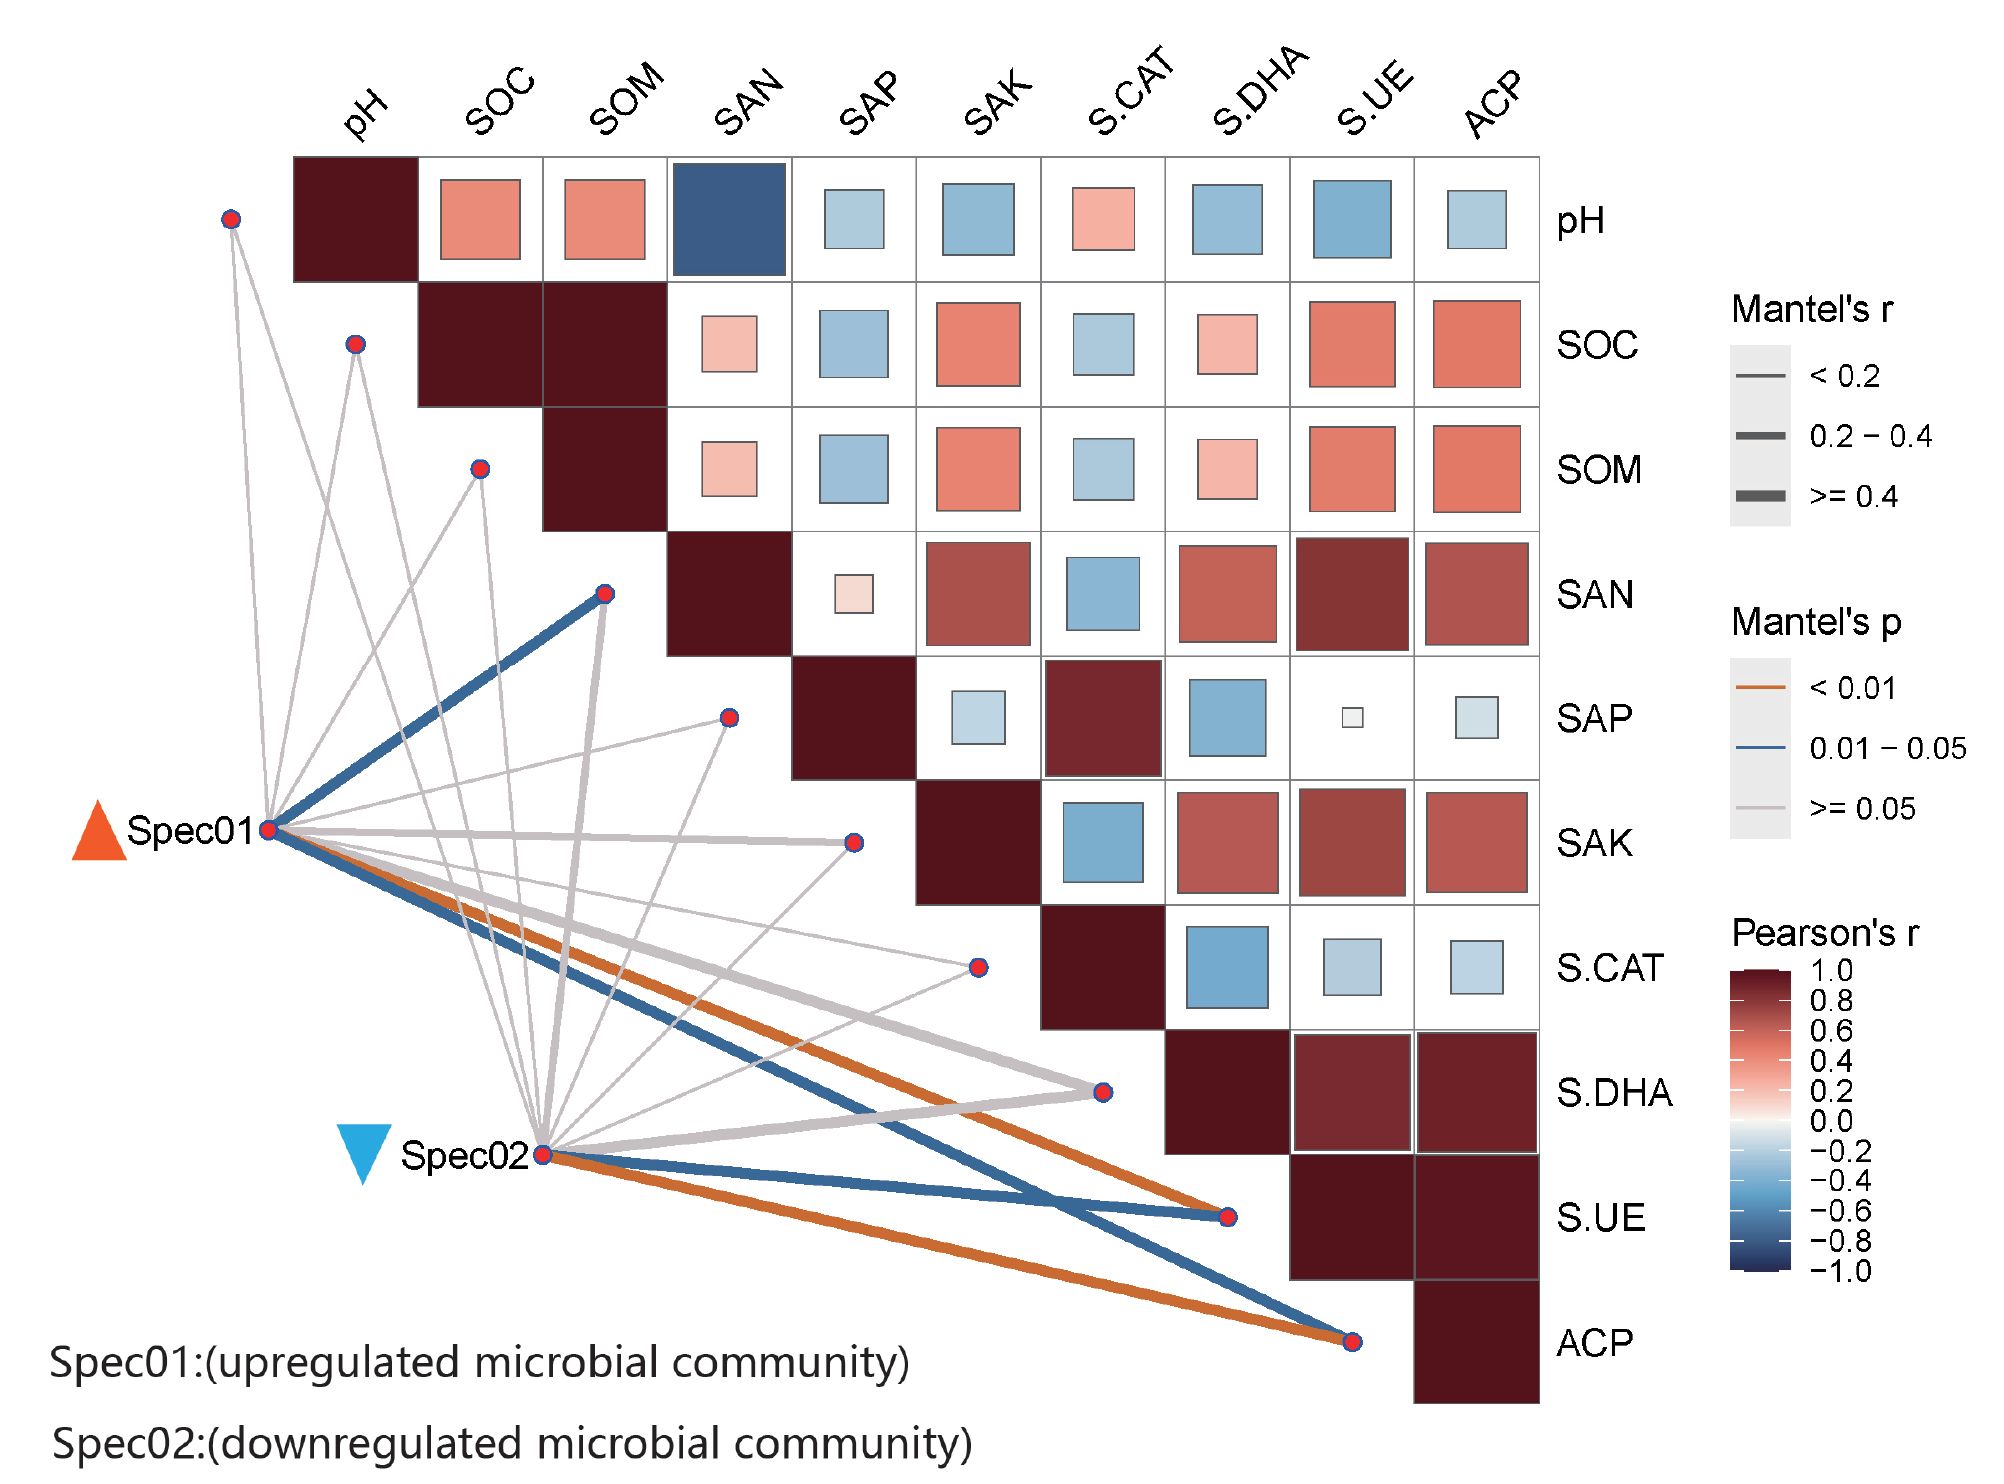
To explore the relationship between the measured environmental factors and the bacterial community, we initially conducted a Pearson correlation analysis of soil environmental factors (Fig. 5). The heatmap showed a negative correlation between pH and soil alkaline hydrolyzable nitrogen (SAN). Furthermore, SAN was positively correlated with soil-available potassium (SAK), dehydrogenase activity (S.DHA), urease activity (S.UE), and acid phosphatase activity (ACP). Soil-available phosphorus (SAP) displayed a positive correlation with catalase activity (S.CAT). Moreover, SAK showed positive correlations with S.DHA, S.UE, and ACP. Notably, the four soil enzyme activities showed strong correlations. Specifically, S.DHA was positively correlated with S.UE and ACP, S.UE showed a positive correlation with ACP, and S.CAT displayed a negative correlation with S.DHA. Building upon the previous analysis at the genus-level analysis, we identified significantly different genera and segregated them into upregulated and downregulated groups. Subsequently, we performed a correlation analysis with the environmental factors. The upregulated genera demonstrated highly significant positive correlations (P < 0.01) with S.UE, significant positive correlations (0.01 < P < 0.05) with SAN and ACP, and a strong positive correlation with S.DHA. On the other hand, the downregulated genera exhibited highly significant negative correlations (P < 0.01) with ACP, significant negative correlations (0.01 < P < 0.05) with S.UE, and a strong negative correlation with S.DHA. Therefore, three soil enzyme activities (S.DHA, S.UE, and ACP) and SAN emerged as crucial environmental factors distinguishing the upregulated microbial community (Spec01) from the downregulated microbial community (Spec02). Since soil enzymes were predominantly synthesized by soil microorganisms, the composition of the bacterial community was significantly influenced by SAN.
Changes in Soil Microbial Functional Characteristics
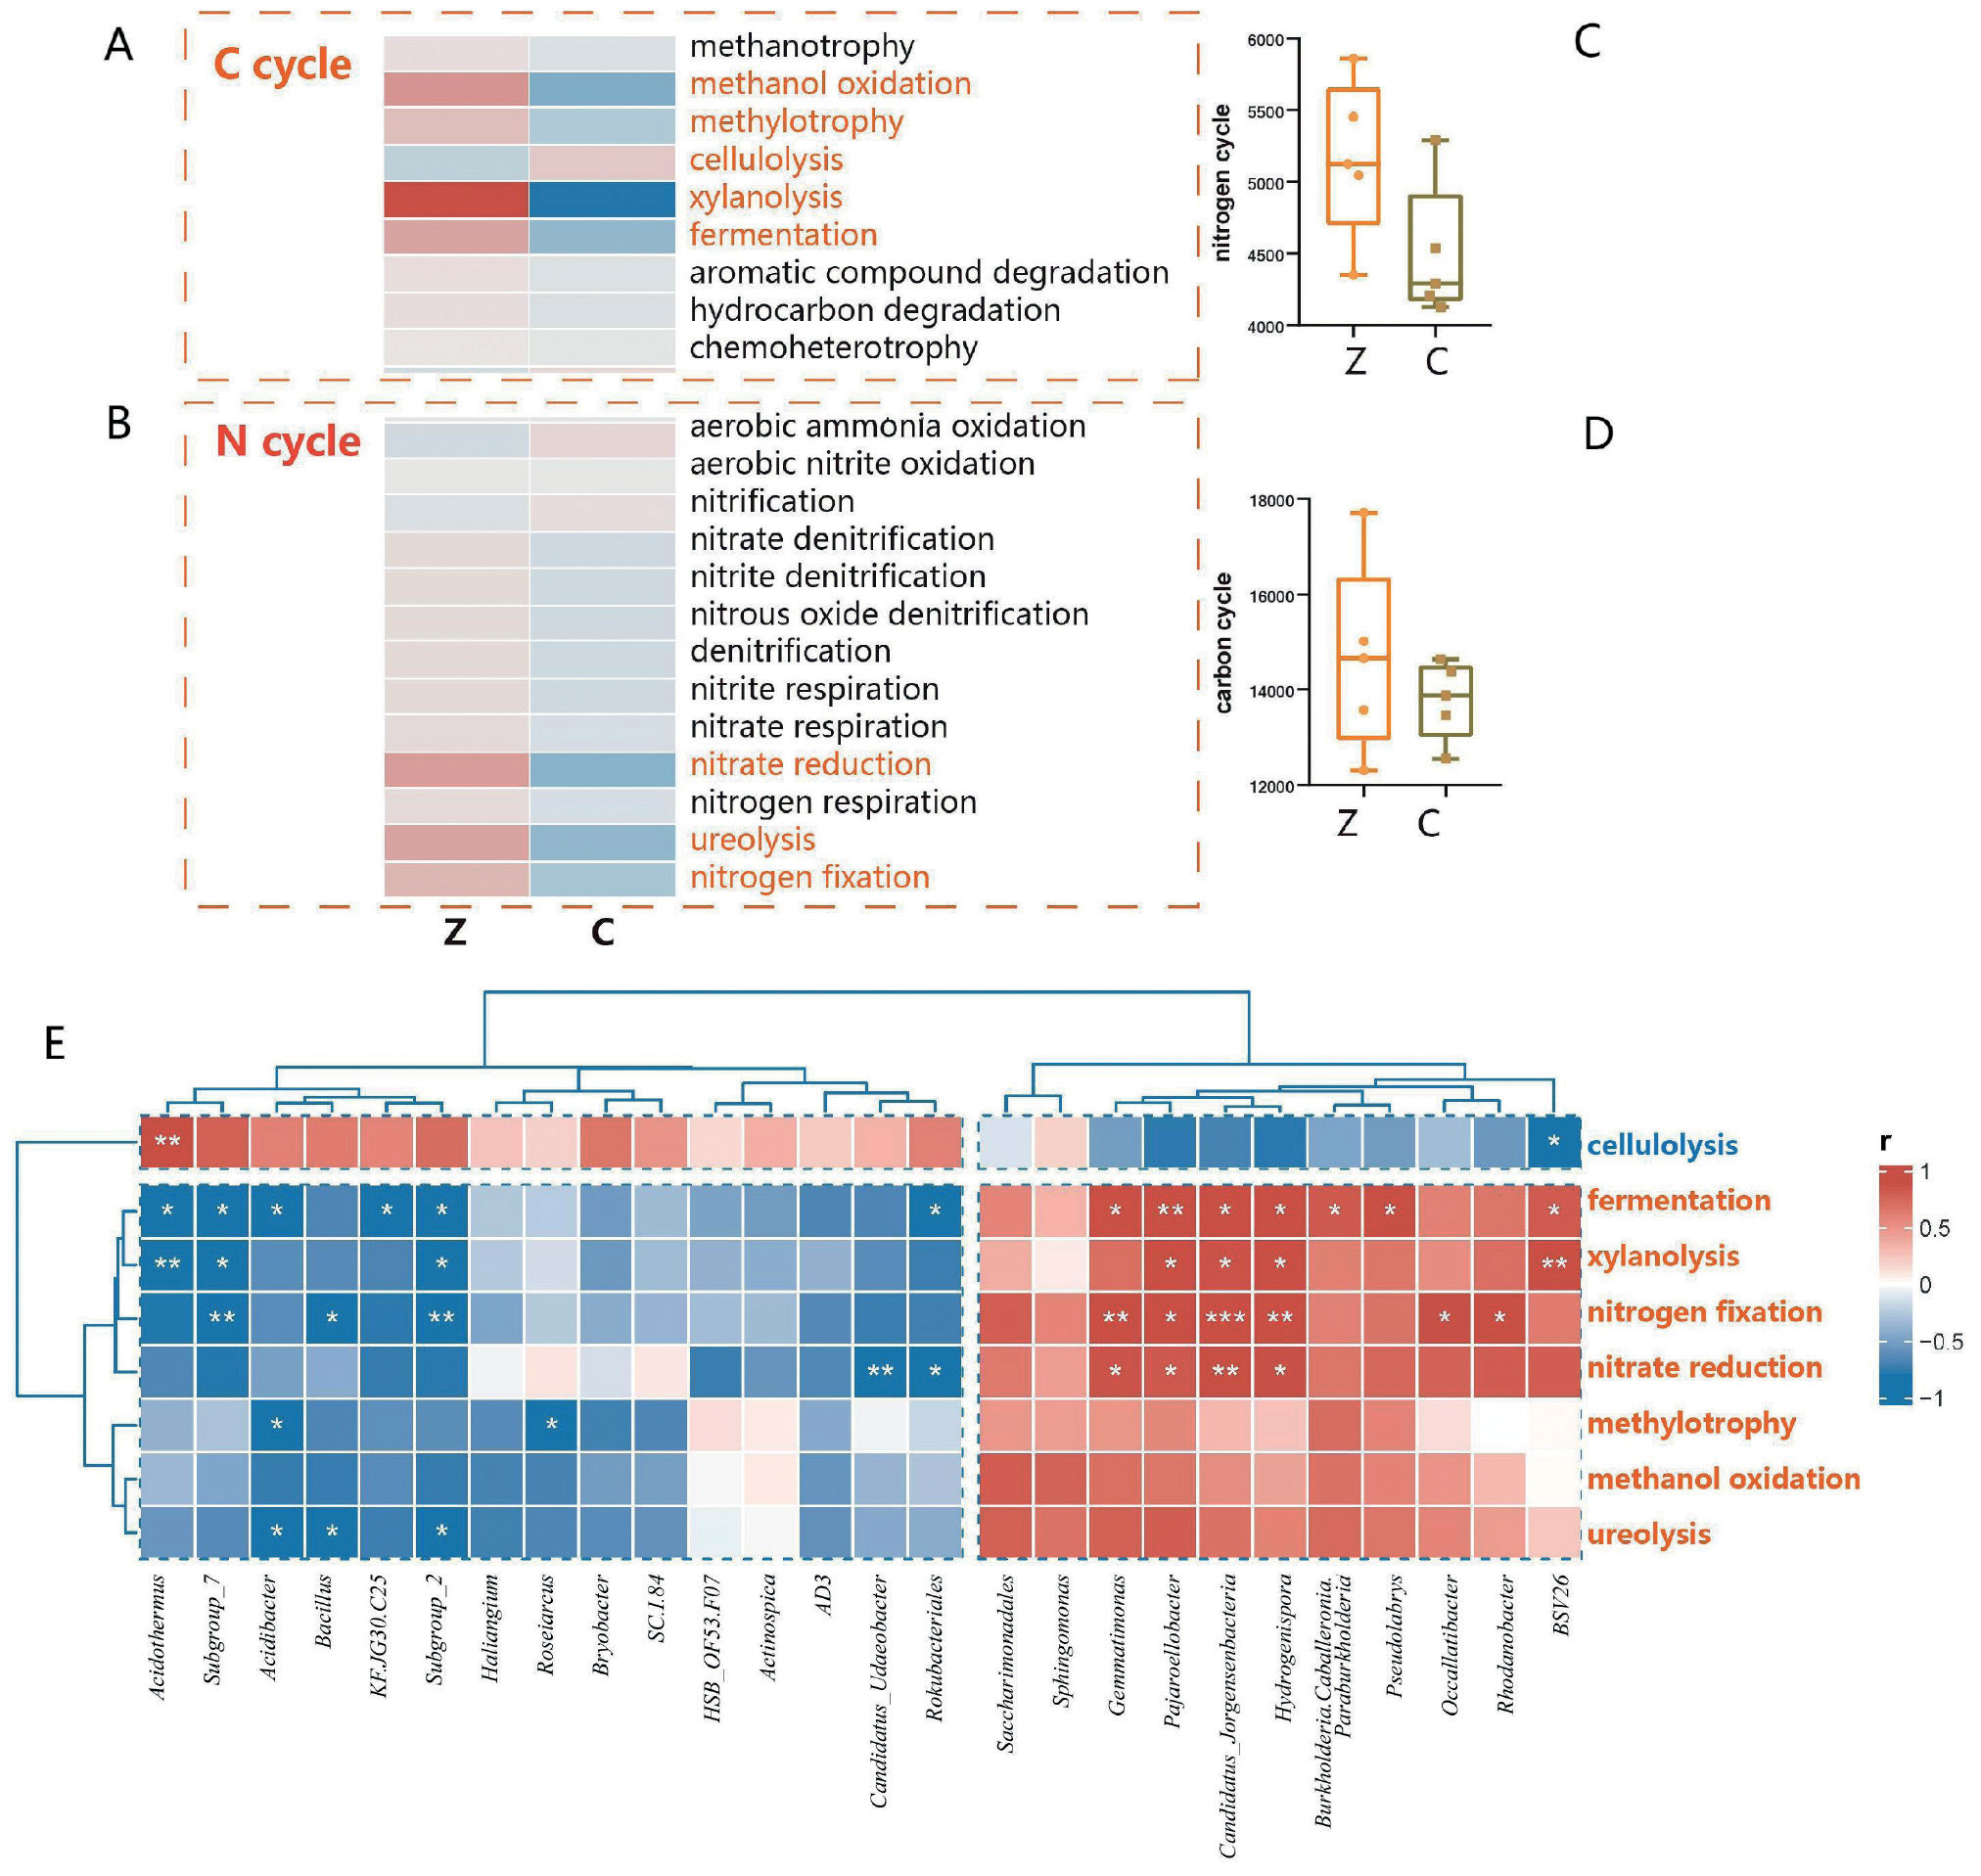
To investigate the impact of intercropping treatments on the functional capabilities of the bacterial community, FAPROTAX analysis was performed. The analysis revealed that nine microbial functions related to the carbon cycle (Fig. 6A) and thirteen microbial functions related to the nitrogen cycle (Fig. 6B) were identified. Compared to the monocropping treatment, five microbial functions involved in soil carbon cycling showed significant differences in the intercropping treatment. Methanol oxidation, methylotrophy, xylanolysis, and fermentation functions were significantly upregulated, while cellulolysis function was significantly downregulated. Additionally, three microbial functions involved in soil nitrogen cycling exhibited significant differences, with nitrate reduction, ureolysis, and nitrogen fixation functions being significantly upregulated. Furthermore, we examined the abundance of microorganisms participating in carbon and nitrogen cycling. The boxplots (Fig. 6C, 6D) clearly demonstrated a significant increase in the abundance of microorganisms participating in these functions in the intercropping group.
Subsequently, we conducted a correlation analysis between the different microbial functions and bacterial genera. The resulting correlation heatmap visually represented these relationships. When comparing the intercropping group to the monocropping group, we observed that the upregulated bacterial group (Spec01) in the intercropping group generally exhibited positive correlations with the upregulated microbial functions. Conversely, the downregulated bacterial group (Spec02) in the intercropping group generally exhibited negative correlations with the upregulated microbial functions. Among the significantly different biological functions, only the cellulolysis function showed downregulation. It demonstrated a highly significant positive correlation with Acidothermus while showing a significant negative correlation with BSV26. The xylanolysis and fermentation functions, both related to the carbon cycle, showed significant positive correlations with the genera Gemmatimonas, Pajaroellobacter, Candidatus_Jorgensenbacteria, Hydrogenispora, and BSV26. Specifically, Pajaroellobacter showed a highly significant positive correlation with fermentation, while BSV26 showed a highly significant positive correlation with xylanolysis. Furthermore, these two functions showed significant negative correlations with Acidothermus, Subgroup_7, and Subgroup_2. Specifically, Acidothermus exhibited a highly significant negative correlation with xylanolysis. The nitrate reduction and nitrogen fixation functions, linked to the nitrogen cycle, showed significant positive correlations with the genera Gemmatimonas, Pajaroellobacter, Candidatus_ Jorgensenbacteria, and Hydrogenispora. Of particular interest, nitrogen fixation showed a highly significant positive correlation with these genera, while exhibiting a highly significant negative correlation with Subgroup_7 and Subgroup_2.
Fig. 6.
Heatmap illustrating the relative abundance of microorganisms involved in soil carbon cycling (A) and soil nitrogen cycling (B) under different planting modes. Boxplots representing the bacterial abundance associated with carbon cycling (C) and nitrogen cycling (D). Heatmap showcasing the correlation between bacterial genera exhibiting significant differences and microbial functions displaying significant differences (E).
Discussion
The management strategy of intercropping in tea gardens can significantly influence soil fertility, which is impacted by various factors, including soil organic matter [29]. Intercropping with D. indusiata and tea trees has been found to enhance the soil organic matter content and improve different soil nutrient indicators to varying degrees. Additionally, this practice also led to alterations in certain physical properties of the soil, such as increased field water-holding capacity and improved soil texture (Fig. 1). These changes in soil environmental factors play a crucial role in reshaping the structure and function of the soil bacterial community [30]. The analysis of α-diversity of the bacterial community, represented by the Chao1 index, Shannon index, and Simpson index, indicated significant increases (Fig. 2A, 2C, 2D), suggesting that the intercropping treatment involving D. indusiata and tea trees effectively enhanced the richness and diversity of the soil bacterial community. Furthermore, β-diversity analysis clearly distinguished the bacterial communities between the intercropping and monoculture groups. The shared soil bacterial OTUs between these two groups accounted for only 14.4% of the total, and changes in the relative abundance at the phylum and genus levels also indicated significant effects of the intercropping treatment on the soil bacterial community structure (Fig. 2F, 2G).
The interactions between soil properties and soil microorganisms are reciprocal and complex, involving causal relationships and feedback networks. Soil microorganisms play a crucial role not only in nutrient cycling and organic matter transformation but also in modifying the soil habitat through biochemical and biophysical mechanisms [31]. Following intercropping treatment, the soil texture transitioned from sandy loam to loam, accompanied by a significant increase in the field water-holding capacity. The activities of four measured soil enzymes, excluding S.CAT, showed significant increases, indicating the involvement of microorganisms in these changes (Fig. 1). Moreover, the increased enzyme activity and microbial biomass have positive implications for soil organic carbon sequestration [32]. Intercropping practices can augment soil moisture content and facilitate the decomposition of soil organic matter. In this study, the intercropping treatment group demonstrated a significant improvement in field water-holding capacity. Enzymes secreted or released by microorganisms, roots, and soil fauna play a crucial role in soil organic matter decomposition [33]. Soil enzymes drive important biochemical reactions involved in nutrient cycling and the breakdown of organic and exogenous nutrients, making them sensitive indicators of soil fertility [34]. Higher enzyme activity indicates an accelerated turnover rate of soil nitrogen and carbon, thereby enhancing soil fertility, consistent with previous studies [35, 36].
Soil properties, such as organic carbon, nutrient availability, texture, and moisture, along with microbial communities, including composition, biomass, and physiological status, play crucial roles in driving the production and turnover of extracellular enzymes in the soil [37]. Intercropping practices have been shown to improve microbial nutrient resources, and the availability of soil nutrients, such as organic matter, alkaline nitrogen, and available phosphorus, is significantly correlated with the abundance of microbial taxa rather than pH values [38]. Consistent with these findings, our study observed no significant difference in soil pH between the intercropping and monocropping groups. However, the bacterial community structure underwent significant changes, indicating that the alterations were primarily driven by variations in soil nutrients. Of particular importance, soil nitrogen content exerted a considerable influence on the bacterial community structure [39]. Modifications in soil nutrient resources can further induce shifts in microbial ecological strategies [39]. From the perspective of microbial community changes, copiotrophic bacteria, represented by Proteobacteria, Bacteroidetes, and Gemmatimonadetes phyla, exhibited increases, while oligotrophic bacteria, represented by Acidobacteria and Nitrospirae, experienced decreases (Fig. 3). This observation suggested that intercropping treatments in tea gardens prompt a transition of microorganisms from oligotrophic to copiotrophic taxa.
Moreover, the observed changes in microbial ecological strategies are supported by predictions of microbial functional potential. Analyses using FAPROTAX for microbial functional prediction revealed significant differences in functional categories related to the carbon cycle, such as methanol oxidation, methylotrophy, xylanolysis, fermentation, and cellulolysis, as well as functional categories related to the nitrogen cycle, including nitrate reduction, ureolysis, nitrogen fixation (Fig. 6). Notably, cellulolysis demonstrated a significant upregulation in its expression. Correlation analysis highlighted a strong and positive association between cellulolysis and Acidothermus. Acidothermus is a cellulose-degrading bacterium that thrives in thermophilic and acidophilic environments, with the ability to produce cellulases that break down cellulose into smaller glucose molecules. Acidothermus cellulolyticus, in particular, has garnered attention due to its cellulose-degrading capabilities. Therefore, the decrease in cellulolysis is directly linked to the decrease in Acidothermus abundance.
The genus Pajaroellobacter, which exhibited a significant enrichment, showed a strong positive correlation with xylanolysis, fermentation, nitrogen fixation, and nitrate reduction. While Pajaroellobacter has been previously identified as a denitrifying bacterium involved in nitrate reduction reactions, no reports have been found concerning its involvement in other functional categories [40]. Therefore, the increase in nitrate reduction functionality can be partially attributed to the increased abundance of denitrifying bacteria, such as Pajaroellobacter. Interestingly, the abundance of Nitrospira, another denitrifying bacterium, showed a slight decrease. This discrepancy may be due to the fact that Pajaroellobacter belongs to the copiotrophic phylum Proteobacteria, while Nitrospira belongs to the oligotrophic phylum Nitrospirae. The changes in soil nutrient resources have likely altered microbial ecological strategies, leading to alterations to the structure of denitrifying bacterial communities.
In the predictions of carbon cycle-related functions, we observed that xylanolysis, the degradation of hemicellulose, significantly increased in the intercropping group compared to the monocropping group. In contrast, cellulolysis, the degradation of cellulose, showed a significant decrease. This difference can be attributed to the change in microbial ecological strategies resulting from the alterations in nutrient resources. Oligotrophic taxa, characterized by slower growth rates and higher substrate affinity, had greater efficiency in decomposing recalcitrant carbon. On the other hand, copiotrophic taxa, with lower substrate affinity, preferentially decomposed easily decomposable carbon [41, 42]. Cellulose, composed of glucose units, is an organic macromolecule with high strength and stability, making it difficult to degrade. Xylan, the main component of plant hemicellulose, has a relatively lower molecular weight and weaker stability, resulting in easier decomposition [43]. In the intercropping system, copiotrophic taxa tend to aggregate and preferentially decompose easily decomposable substrates due to changes in nutritional strategies. As a result, the xylanolysis function was enhanced, while cellulolysis significantly decreased. In addition, previous research had indicated a clear correlation between xylan degradation and certain members of the phylum Bacteroidetes, particularly Bacteroides xylanisolvens XB1A (BX) [43]. These bacteria encode endoxylanases Xyn10A and Xyn10B, which are responsible for degrading the main xylan chain within genes PUL43 and PUL70, respectively. Furthermore, most Bacteroidetes strains contain two xylanases in their genomes, suggesting that Bacteroidetes are the primary taxonomic group involved in xylan degradation [44, 45]. However, in the intercropping system, while the relative abundance of the phylum Bacteroidetes significantly increased, there was no precise identification of changes in the abundance of Bacteroides specifically. Instead, there was a significant increase in the relative abundance of the genus BSV26. However, research on the lignin degradation ability of BSV26 is limited, with only one study suggesting its dominance in lignocellulosic degradation systems [46]. Therefore, we can only speculate that the increase in xylan degradation is associated with the increased abundance of copiotrophic taxa, such as Bacteroidetes. Hydrogenispora, an anaerobic carbohydrate-fermenting bacterium derived from anaerobic sludge, belongs to the phylum Firmicutes and is an important representative of the copiotrophic group. It plays a significant role in natural biodegradation and carbon cycling [47–49]. Therefore, the increase in the abundance of this genus contributes to the overall promotion of carbon cycling.
Significant increases in the relative abundance of rhizosphere-promoting bacteria, including Gemmatimonas, Sphingomonas, and Burkholderia-Caballeronia-Paraburkholderia were observed in the intercropping treatment. Burkholderia-Caballeronia-Paraburkholderia is a nitrogen-fixing bacterium [50] that not only fixes atmospheric and soil nitrogen but also produces hormones and metabolites such as indole- 3-acetic acid, gluconic acid, and glucosamine. These compounds stimulate root development, increase plant biomass, and improve plant yield. They also produce antimicrobial substances that inhibit or kill some plant pathogens, enhancing plant resistance to diseases [51, 52]. Similarly, Sphingomonas, another rhizosphere-promoting bacterium, plays a role in nitrogen fixation and promotes crop root growth [53, 54]. This bacterium produces auxins, nitric oxide, and iron carriers, and displays ACC deaminase activity. It also regulates other plant hormones, such as abscisic acid, jasmonic acid, and salicylic acid, which are crucial for plant development and defense responses. Some strains of Sphingomonas have been shown to improve plant nitrogen supply by forming functional root nodules. Moreover, Sphingomonas species are known for their ability to degrade various organic compounds, including polycyclic aromatic hydrocarbons, pesticides, and organic waste. Furthermore, Gemmatimonas, in the correlation analysis, showed positive correlations with multiple functions in carbon and nitrogen cycling. While most research on Gemmatimonas focused on its ability to solubilize insoluble phosphorus and convert it into available phosphorus for plant growth, induce plant stress tolerance, or produce antifungal antibiotics [55, 56], it had been found that Gemmatimonas can also respond to changes in soil nutrient content [57]. However, relatively less research has been conducted on its involvement in carbon and nitrogen cycling.

