

Introduction
Plant functional traits are a result of the interplay between natural selection and environmental filtering. They provide valuable insights into the role of biodiversity in ecosystem functioning and how ecosystems respond to environmental disturbances [1-4]. Functional traits associated with ecosystem functions are often linked to resource acquisition, plant size, and regeneration [1, 2]. These traits have a profound impact on primary productivity and carbon cycling. Consequently, it is crucial to quantify the relationship between environmental factors and plant functional traits in order to enhance our understanding of plant adaptation to different environment [5].
Submerged plants play a vital role in wetland ecosystems as they occupy crucial ecological niches at the water-sediment interface [6-8]. They contribute significantly to the regulation of material cycling and energy transfer in lake and river ecosystems. Submerged plants provide shelter and food for organisms, reduce phytoplankton biomass through allelopathy, remove nutrients from water, and control sediment resuspension [9-11]. Due to the unique physicochemical properties of aquatic environments, submerged plants face more complex and diverse habitats, as well as various selection pressures. These results in the development of distinct structural, physiological, growth, and reproductive characteristics. For instance, submerged plants have the ability to disperse through seeds, creeping branches and plant fragments, with the latter being particularly effective in facilitating medium- to long-distance transmission, enhancing reproductive success, and reducing predation risk [12, 13].
The worldwide issue of eutrophication in lakes has led to the proliferation of harmful algal blooms and decline, and even extinction of aquatic plant. Submerged plants play a crucial role in promoting the transition of lake ecosystems from turbid water state to clear water state through their structural effects [14]. They are key players in maintaining the stability of clear water conditions in lakes. The growth and decline of submerge plants directly impact the functioning of lake ecosystems and vital for regulating lake eutrophication. The successful reconstruction and preservation of submerged plants are pivotal in the rehabilitation of shallow eutrophication lakes. The rapid and effective restoration and reestablishment of submerged vegetation have become significant scientific and technological challenges in lake and reservoir management.
Sediment serves as a fundamental requirement for submerged plants to established roots, reproduce, and grow steadily. It is also acts as a direct sources of nutrients, significantly influencing biomass accumulation, root morphology, root distribution, and nutrient concentrations in submerged plants [12, 15- 17]. In response to nutrient heterogeneity, plants can modify root architecture (e.g., root length, root diameter, and root mass) and other morphological characteristics (e.g., shoot to root mass ratio) [13, 18]. However, the effects of sediment heterogeneity and planting density on submerged plant traits remain unclear, particularly regarding the potential interaction effects and their extent.
Myriophyllum spicatum is a cosmopolitan submerged aquatic macrophyte widely distributed worldwide. It is highly valued in the field of water treatment due to its ability to produce a large amount of biomass and its fast growth rate. Both domestic and international research on M. spicatum in water treatment primary focuses on four areas: biosorption, biodegradation, bioenergy utilization and ecotoxicology [19-22]. One key aspect of M. spicatum that is of interest in water treatment is its ability to adsorb heavy metals and organic pollutants. The cell surface of M. spicatum possesses abundant functional groups, such as hydroxyl, carboxyl, and collagen proteins, which enable it to adsorb these contaminants. Researchers are actively working on enhancing the adsorption efficiency of M. spicatum for pollutants by optimizing cultivation conditions and manipulating algal cell characteristics. Additionally, M. spicatum plays a crucial role in the oxygen-carbon dioxide cycle. During photosynthesis, it releases oxygen into the water while absorbing carbon dioxide. This process contributes to maintaining the balance of dissolved gases in aquatic ecosystems and helps mitigate the negative effects of excessive carbon dioxide levels. Due to its high biomass production and lipid content, researchers are investigating the potential of M. spicatum for biofuel or biogas production. Several studies have already explored techniques for biomass conversion and lipid extraction from M. spicatum. As an aquatic plant found in various water bodies, M. spicatum exhibits specific ecotoxicological responses to pollutants present in water. Researchers evaluate the growth and physiological indicators of M. spicatum in polluted environments to assess water pollution levels and determine the biological toxicity. These studies contribute to the understanding of the impact of pollutants on aquatic ecosystems and help in developing effective remediation strategies. In summary, research involving M. spicatum extends beyond its adsorption capabilities, encompassing the potential for biofuel production, ecotoxicology assessment, and water pollution evaluation. The versatility and adaptability of M. spicatum make it an attractive candidate for multiple applications in the field of water treatment and ecological restoration [19-22].
Fragments generated through the natural shedding of plant tops and environmental disturbances can give rise to new plants [13, 23]. This mechanism holds significant importance in the reproduction and expansion of plant populations [24]. Fragment colonization is influenced by a combination of biotic and abiotic factors, making it challenging to predict the outcome solely based on a single factor [13, 25]. When it comes to the colonization of fragments, the interplay of various biological and environmental factors comes into play. In this study, we conducted an indoor cultivation experiment to explore the morphology and biomass characteristics of M. spicatum under different planting densities of 1 plant/pot, 10 plants/pot. Furthermore, we also examined the effects of sediment heterogeneity, specifically different sediment types including mud, upper sand + lower mud, sand, and upper mud + lower sand. We evaluated how these variations in sediment type and density influenced the growth of M. spicatum.
Material and Methods
Shoots of M. spicatum were collected from Huixian Karst Wetland in Guilin. Upon transporting them to the laboratory, apical shoots with comparable basal stems were carefully chosen. These selected shoots were then cut into 12 cm fragments to prepare them for pre-cultivation. The fragments were buried at a depth of 2 cm in a plastic pot (120 L, 55 cm high) containing a layer of sand at the bottom. The pots were then filled with water and placed outdoors to receive natural sunshine. After pre-incubation period of 7 days, adventitious roots started to grow on the cultivated fragments. Subsequently, the fragments were transplanted into PVC pots with 12 cm in diameter and 10 cm in height. There were four types of sediments (Fig. 1): 12 cm clay (short for I), sand 6 cm + clay 6 cm (short for II), sand 12 cm (short for III), clay 6 cm + sand 6 cm (short for IV). Two planting densities were applied, with 1 plant per pot and 10 plants per pot. Each habitat and planting density combination had 5 replicates per density for each habitat, and then put into plastic tanks filled with water, all in 3 tanks, 180 pots. To avoid impacts of algae growth on the fragment, water in tanks were changed every 3 days. Plants were harvested after 45 days.
Before planting, the biomass of each fragment was measured for later calculation of relative growth rate (short for RGR) and relative elongation rate (short for REG). RGR and RER were calculated as follows [13]:
RGR = (lnw2 − lnw1)/ (t2 − t1)
RER = (lnh2 − lnh1)/ (t2 − t1) where w1 is the initial dry mass, w2 is the dry mass at harvest time t2, h1 is the initial height, h2 is the height at harvest time t2, and (t2 − t1) is the experimental time.
During the harvesting process, plant roots were delicately extracted from the sediment and rinsed with tap water. The basal stem was measured using a Vernier caliper, while height was measured with a ruler with a 0.1 cm precision. Following these measurements, plants were separated into aboveground and underground parts, and their fresh weights were measured separately. Subsequently, the plant samples were placed in an oven at 80ºC for 72 h, and then weighed again to determine the dry weights. The plant biomass was calculated by summing of the aboveground and underground parts.
The normality and homogeneity of variance for all the data were assessed using Shapiro-Wilk normality test. Two-way analysis of variance was conducted to analyze the basic stem, relative growth rate, relative elongation rate, above-ground biomass, under-ground biomass, and total biomass of M. spicatum across different planting density (1 plant/pot and 10 plants/pot) and four sediment types. The significance level set at p<0.05. All data processing and graphical representation were performed using SPSS 22.0 and Graphpad Prism 8.0, respectively.
Results
Effects of Planting Densities and Sediment Types on Morphological and Biomass Traits
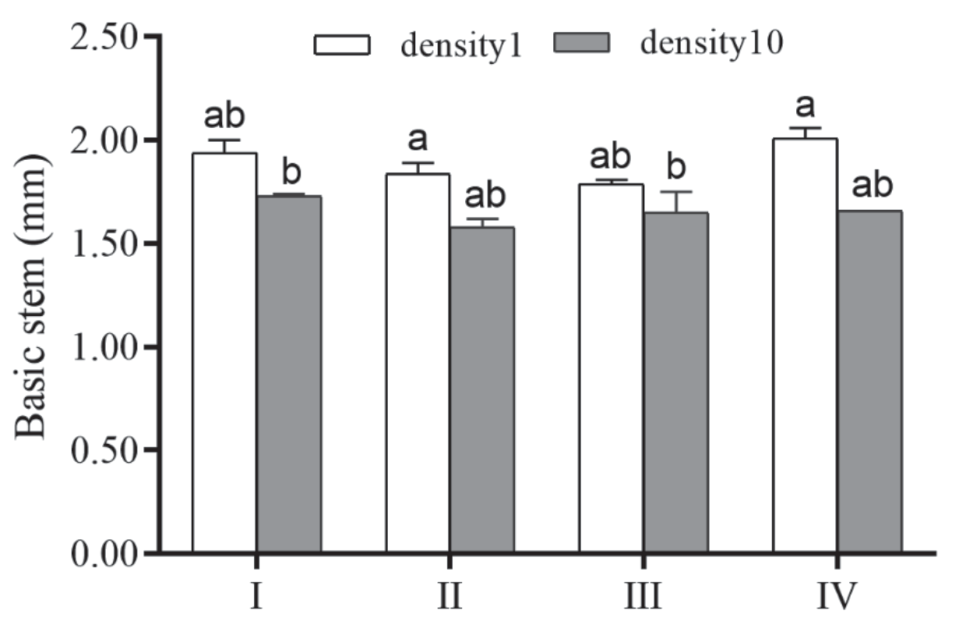
Planting densities had no significant effect on the basic stem of M. spicatum (Table 1; Fig. 2). Basic stem of density 1 was bigger than density 10 in all four sediment types. However, the influence of sediment type on the base stem is not consistent with the planting density. There is no significant difference in basal stem among different sediment types in density 1 or density 10.
The highest and lowest relative elongation rate all occurred in density 1, with the highest in sediment type II and the lowest in sediment type I (Table 1; Fig. 3a). In density 10, except for the significant difference in relative elongation between sediment I and III, the differences between the other several are not significant. Therefore, planting density had no significant influence on the relative elongation rate.
Fig. 1.
Experimental scheme, showing the four sediment types (clay; sand+ clay; sand; clay+ sand) and two planting densities. Each treatment was conducted with five replications.
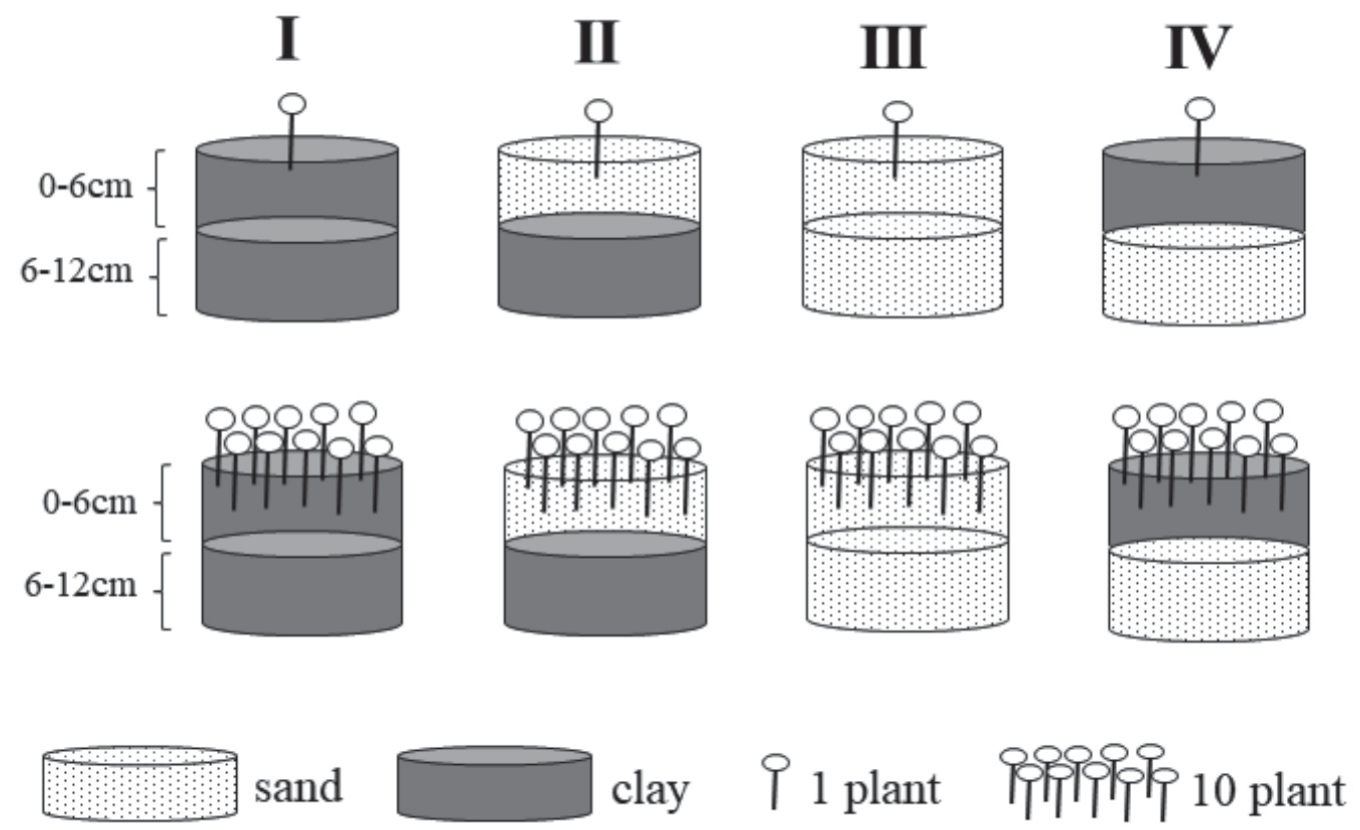
Table 1.
Two-way analysis of variance for the basic stem, relative growth rate, relative elongation rate, above-ground biomass, under-ground biomass, and total biomass of M. spicatum with different planting densities grown in four sediment types.
Fig. 2.
Basic stem of M. spicatum in different planting density and sediment types (mean±SE). Bars sharing the same letters indicate no significant differences among treatments (p>0.05) and the different letters indicate significant differences among treatments (p<0.05).
Relative growth rate was only affected by planting density (Table 1; Fig. 3b). Among the different sediment types in density 1, sediment type III exhibits the highest relative growth rate, with no significant difference observed compared to sediment II and IV. In contrast, sediment type I demonstrates the lowest relative growth rate, with significant differences observed compared to the other three sediment types. Similarly, in density 10, sediment type III also exhibits the highest relative growth rate, but there is no significant difference observed among the four sediment types. Therefore, when compared to planting density, the influence of sediment type on relative growth rate is not particularly significant.
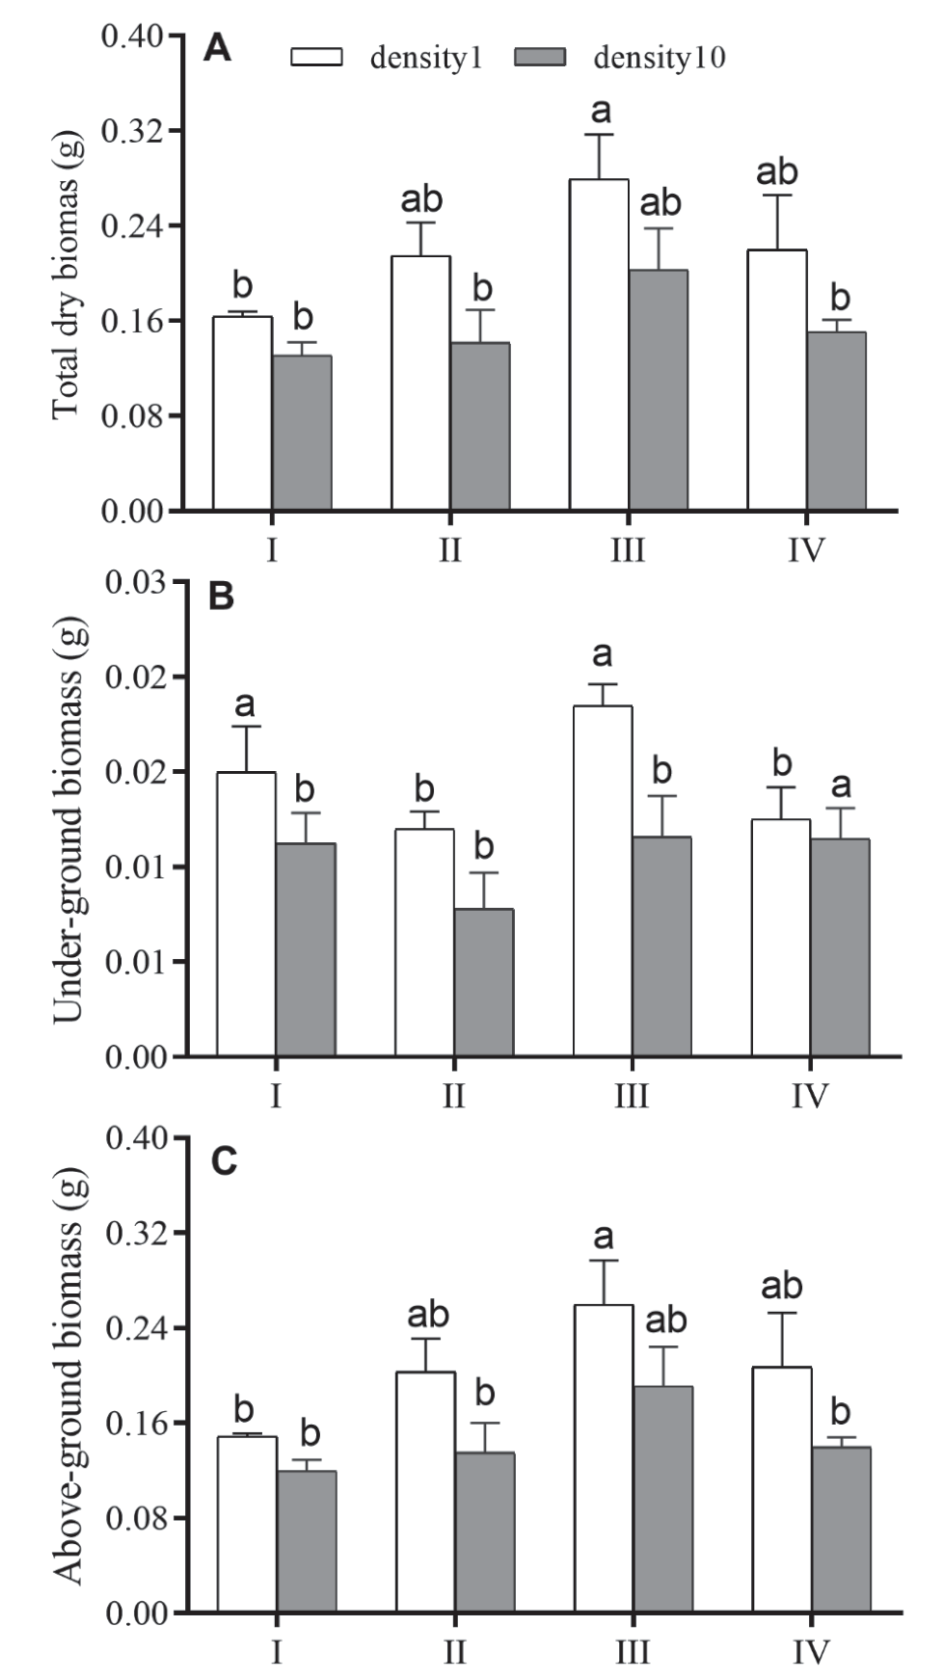
The analysis of above-ground biomass and total dry biomass revealed that they were only influenced by the variation in sediment type. On the other hand, the under-ground biomass was found to be affected by both sediment types and planting density (Table 1; Fig. 4). The analysis of biomass changes revealed that in both planting densities, the order of fresh weight and dry weight was as follows: II>IV>I>III. The maximum dry weight recorded was 0.28 g/plant, while the minimum was 0.14 g/plant, indicating a maximum difference of 2-fold between the highest and lowest values.
In the case of density 10, after a growth period of 45 days, more than 60% of the biomass in four sediment types exhibited a negative growth trend. This means that the harvest fresh weight was lower than the initial planting fresh weight. Particularly in sediment type III, the negative growth of plants reached up to 75%, whereas sediment type I exhibited a smaller negative growth rate.
However, in density 1, only sediment type III showed a negative growth pattern, with the other sediment types showing either positive growth or no significant change in biomass.
3.2 Effects of planting densities and sediment types on biomass distribution characteristics
When considering the biomass allocation in the two planting densities, the order of above-ground biomass to total biomass was found to be III>I >IV>II (as shown in Fig. 5). This indicated that sediment III had the highest proportion above-ground biomass, while sediment type II had the lowest proportion. But there is not much variation in the above-ground and under-ground biomass allocation of different sediment types between the two planting densities. These results suggest that sediment type has a more significant influence on biomass allocation than planting density.
Discussion
The environment plays a crucial role in shaping the growth and development of submerged plants. It does not only directly influence their individual growth and morphological but also impacts the distribution of plant communities [26, 27]. Submerged plants have the ability to absorb nutrients from both sediment through their root systems and water through their stems and leaves. This process helps reduce sediment resuspension and improve water clarity, thus exerting a significant influence on the structure, function and system stability of lake ecosystem [28, 29]. A fertile substrate promotes plant tillering, growth and increased biomass. This nutrient uptake from the sediment plays a crucial role in supporting the positive growth and development of submerged plants. It is through this process that submerged plants acquire almost all of their required nitrogen and phosphorus [20].
Fig. 3.
Relative elongation ratea) and Relative growth rate b) of M. spicatum in different density and sediment (mean±SE). Bars sharing the same letters indicate no significant differences among treatments (p>0.05), and the different letters indicate significant differences among treatments (p<0.05).
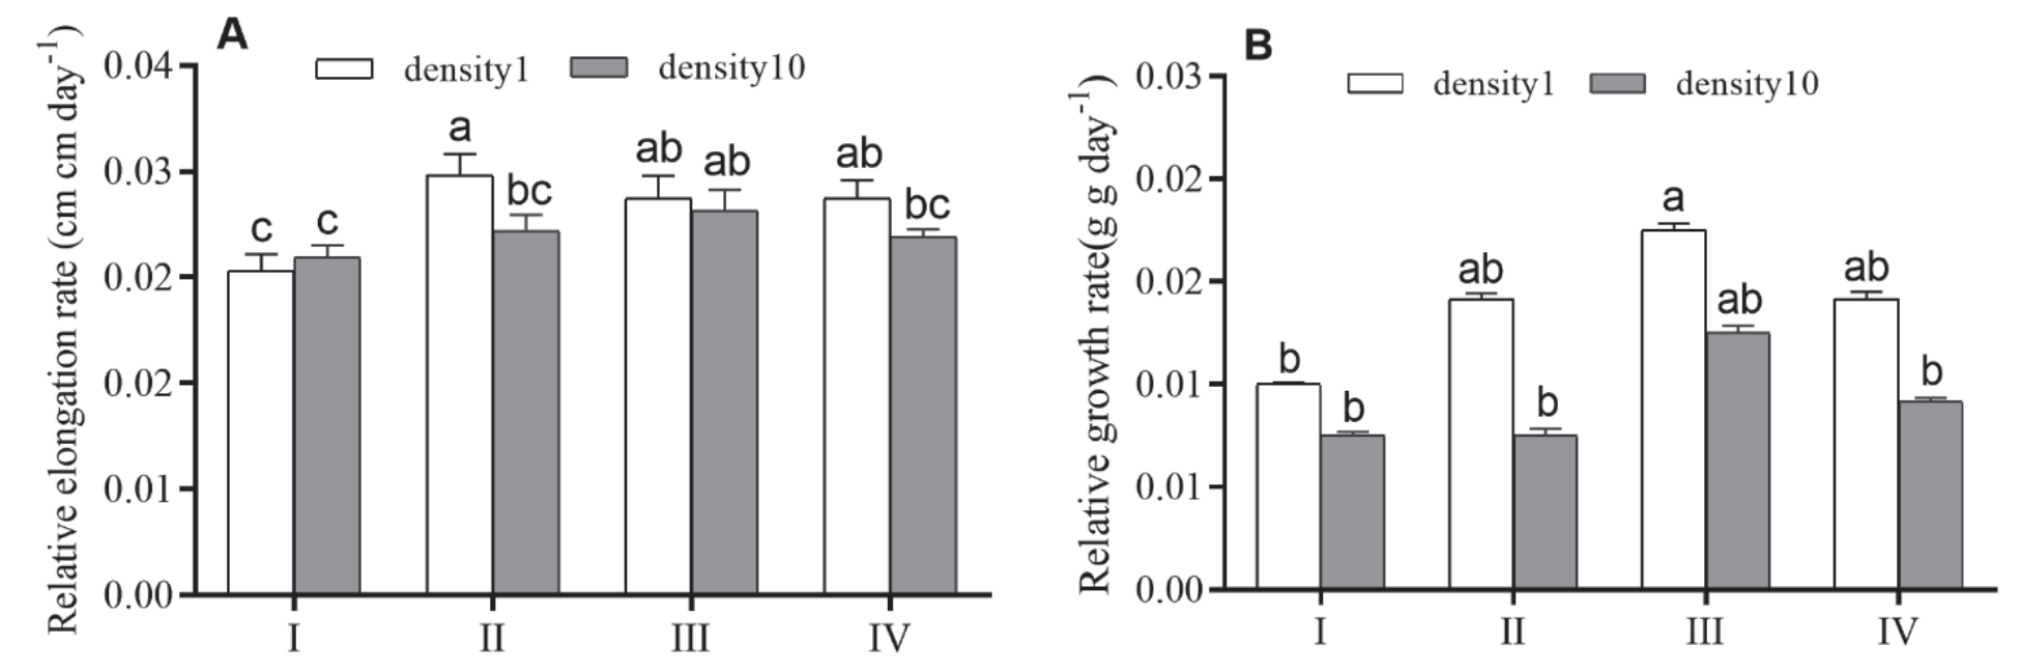
Fig. 5.
Distribution of above-ground and under-ground biomass of M. spicatum in different planting density and sediment types. A-density1, B-density 10.
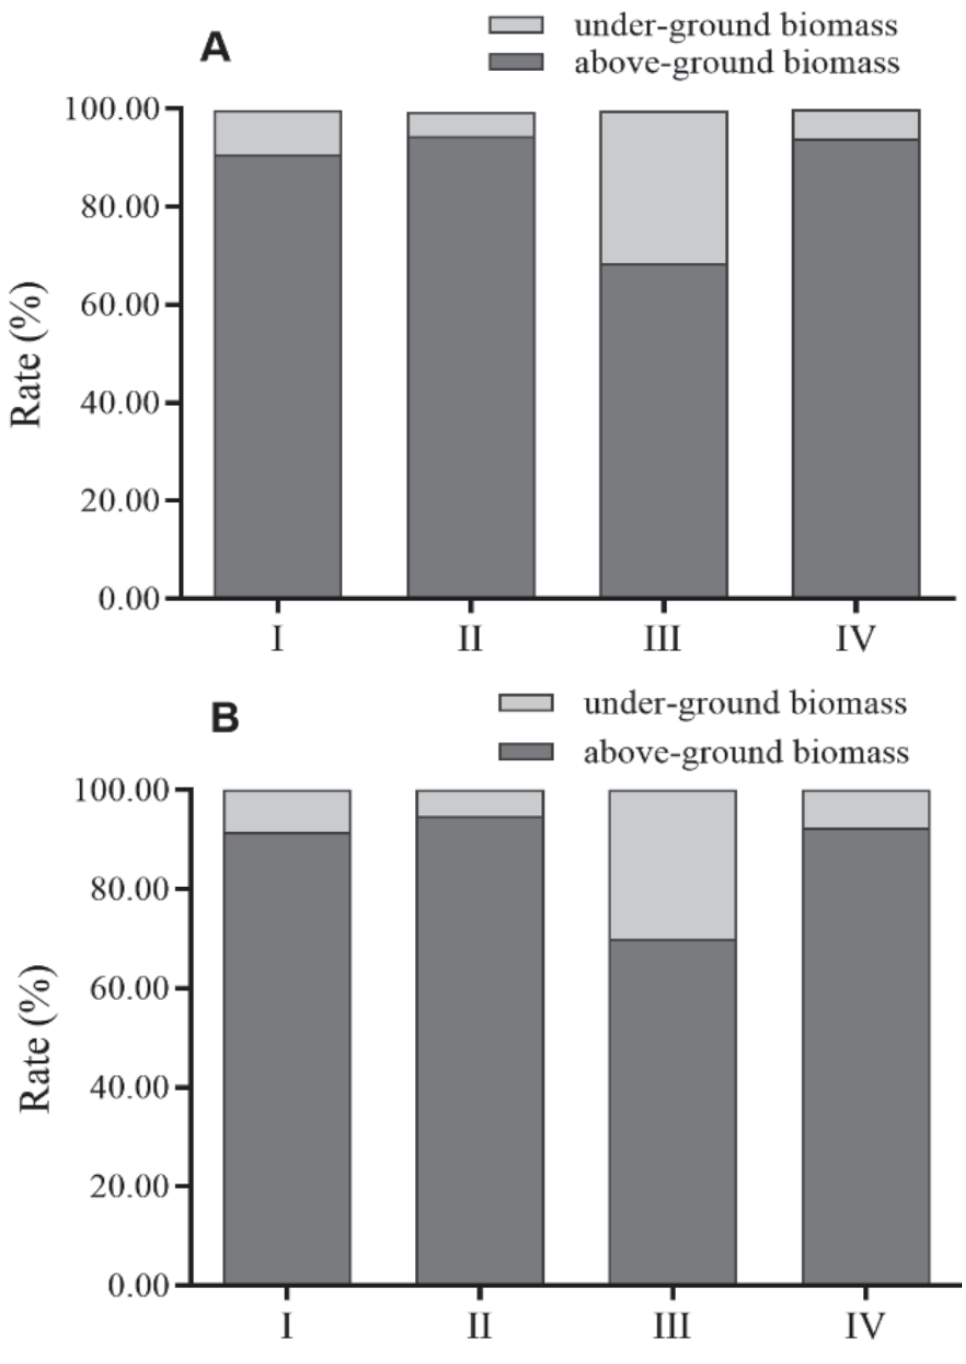
Fig. 4.
Total dry biomass A), Above-ground biomass B), and Under-ground biomass C) of M. spicatum in different planting density and sediment types (mean±SE). Bars sharing the same letters indicate no significant differences among treatments (p>0.05), and the different letters indicate significant differences among treatments (p<0.05).
Plant traits are well-known indicators of how plants respond to environment factors, including nutrient availability and other resources [30]. In wetland plants, roots perform crucial functions such as anchoring, absorbing and conserving water and nutrients, as well as synthesizing and storing nutrients. The growth, distribution and functional characteristics of roots adapt to changes in environmental conditions, which in turn influence the composition and distribution of vegetation communities. In the case of submerged plants, roots play a key role in nutrient uptake from sediment. The structure, density and nutrient content of sediment directly impact root development and, consequently, overall plant growth [31]. The allocation of aboveground and under-ground biomass in M. spicatum is influenced by water quality and light conditions. The above-ground biomass provides shade, slows down water flow, and protects sediment, thereby assisting in preventing sediment erosion. Simultaneously, the under-ground biomass stores a significant amount of organic matter in the sediment, regulating groundwater quality and nutrient cycling in the water. The underground biomass primarily consists of rhizomes and roots, providing better support and stability to help M. spicatum survive and grow under low light conditions. In nutrient-rich and shallow water environments, M. spicatum tends to allocate more biomass to the aboveground portion.
While permeability is favorable for the growth and development of plant roots, the experiment revealed that M. spicatum exhibited the lowest biomass in sediment type I, which consisted of sand, for both densities. In response to the limited nutrient availability in sand sediment, M. spicatum allocated a greater proportion of energy towards subsurface components. This adaptive strategy armed to accelerate root growth and enhance nutrient acquisition from the sediment, thereby improving resources access and increasing biomass to support the species’ requirement for survival and reproduction. These findings indicate that M. spicatum can regulate biomass allocation and root structure in response to oligotrophic habitats. The morphological plasticity exhibited by M. spicatum enables enhanced adaptability to heterogeneous habitats, which contributes to its crucial role as a pioneer species in water restoration projects. Therefore, the allocation of aboveground and belowground biomass in Zostera marina reveals the adaptive strategies and ecological functions of the species under different environmental conditions.
Planting density is an additional crucial factor that influences the reproduction and growth of submerged plants. For instance, Potamogeton perfoliatus tends to produce more branches when planted at lower densities. On the other hand, the height of Atriplex prostrata decreases as the planting density increases [32].
When nutrients are readily available to fulfill the growth requirements of plants, the above-ground biomass increases as more resources are allocated towards the development of organs that capture light. Conversely, there is an increase in under-ground biomass. The total biomass of submerged plants serves as a visual indicator of the growth, health and population development of individual organism [33]. The relationship between biomass and resource efficient indicates that higher biomass allows for greater resource utilization and energy acquisition, resulting in further biomass increase. Conversely, a decrease in biomass suggests increased environmental stress and reduced adaptability of individuals. In this study, it was observed that at density 1, basal stems were larger in all habitats compared to density 10. Furthermore, sediment type III exhibited the smallest net stem elongation and significantly lower net stem elongation and total biomass compared to the other three sediment types, indicating a limited nutrient supply in sediment type III. At density 10, a higher proportion of negative growth in total biomass was observed in all sediment types compared to density 1, particularly in sediment type III. To conclude, in addition to the substrate nutrients, planting density appears to play a significant role in the growth of M. spicatum.
Conclusions
Aside from sediment nutrients, planting density also plays a crucial role in the growth of M. spicatum. In all four sediment types, M. spicatum exhibited superior morphological growth under low-density planting compared to high-density planting. Although planting density had minimal impact on biomass distribution patterns within the same sediment, there but biomass of was a significantly higher biomass in areas with high heterogeneity compared to low heterogeneity. The high morphological plasticity of M. spicatum enables it to adapt effectively to varying habitats, which likely contributes to its importance as a pioneer species in water restoration initiatives.
This study provides a fresh perspective on the morphological plasticity of M. spicatum, highlighting its ability to adapt to varying planting densities and substrate heterogeneity through the modulation of biomass allocation patterns and root morphological. Consequently, the selection of appropriate cultivation sediment and methods become crucial for successful establishment of submerged plant communities in different aquatic environments. These findings provide valuable insights for future research and development of techniques related to the screening, colonization and construction, regulation and management of submerged plant communities. Furthermore, they offer vital technical support for water ecosystem restoration projects.

