

Introduction
Soil saline alkalization is one of the main causes of soil degradation [1]. It has been reported that 20% of the world’s irrigated land is currently affected by saline alkalization, accounting for 25% of the total global cropland area [2]. The area of saline alkalization land in China is about 9.91×10⁷ ha. The increase in soil saline alkalization leads to the deterioration of the ecological environment, which ultimately affects crop yield [3].
Rice (Oryza sativa L.), as a common food crop, is a saline-alkali-sensitive crop, especially during rice seedling and reproductive growth stages [4]. Saline-alkali stress causes osmotic and ionic stress [5], which in turn causes oxidative stress, reduces photosynthesis, and hinders nutrient uptake [6], ultimately inhibiting rice growth and development [7].
The application of various techniques promoted the rapid development of biological research [3, 8]. Metabolomics is a biological technique used to visualize various metabolites in plants at a specific time as well as in a specific environment, especially in stress conditions [9]. Guo et al. [10] analyzed the effects of neutral and alkaline salt stress on wheat metabolism using the GC-MS technique and screened 75 differential metabolites, including organic acids, amino acids, sugars, and polyols. Zhang et al. [11] utilized GC-MS technology to determine the metabolites of low-temperature-stressed rice, and clarified the response of rice to low temperature and the dynamic metabolic modeling of recovery. Chen et al. [12] identified 90 differential metabolites (49 up-regulated and 41 down-regulated) in Dongxiang wild rice under salt stress.
Our earlier studies found that saline-alkali stress affected the physiological metabolism of rice seedlings [13, 14]. However, there are few studies on the dynamics of metabolites in rice seedlings under saline-alkali stress. In this study, we utilized GC-MS to detect the metabolic regulation mechanism in rice seedlings in response to saline-alkali stress and provided the theoretical basis for the future analysis of saline-alkali stress resistance in rice seedlings.
Materials and Methods
Cultivation and Treatment of Materials
Healthy rice seeds (Beijing No. 2) were sterilized with 1% NaClO for 30 min and rinsed with distilled water. Rice seeds were germinated at 28ºC for 24 h, and then 100 germinated seeds were cultured on a plastic beaker (700 mL) containing sterilized Hoagland nutrient solution in a light incubator (day/night temperature of 28/26ºC, light/dark time of 16/8 h, relative humidity of 80%, and light intensity of 10,000 lux), and supplemented daily with Hoagland nutrient solution. Then two leaves-one heart rice seedlings were divided into two groups for treatment, control (CK): cultivated with Hoagland nutrient solution; saline-alkali stress treatment (N): cultivated with Hoagland nutrient solution containing 10 mM Na2CO3. Five biological replicates were set up for each treatment. After 10 d of treatment, growth parameters were determined and aboveground parts were frozen in liquid nitrogen for metabolomics analysis.
Determination of Growth Parameters and Relative Growth Rates
Ten rice seedlings were randomly selected from each treatment and plant height, root length, and dry weight were measured to calculate the relative growth rate.
Relative growth rate (RGR) = [ln (dry weight after stress treatment) - ln (dry weight before stress treatment)]/number of days of treatment
Metabolomics Analysis
Metabolite Extraction
Rice seedling samples (100 mg) were transferred to 5 ml centrifuge tubes and ground by a high-throughput tissue grinder (70 Hz/min), then 1,400 μL of pre-cooled methanol was added and stirred for 30 s. Then, 60 μL of ribitol (0.2 mg/mL) was added as an internal quantitative standard and stirred for 30 s. The samples were placed in an ultrasonic apparatus at room temperature for 30 min, and 750 μL of pre-cooled chloroform and 1,400 μL of deionized water were added and stirred for 60 s and centrifuged for 10 min in a 14000 r/min centrifuge. Pre-cooled chloroform and 1400 μL deionized water (dH2O) were added, stirred for 60 s, and centrifuged for 10 min in a centrifuge at 14000 r/min. 1 mL of the supernatant was concentrated under vacuum and added to 60 μL of methoxylamine pyridine solution (15 mg/mL), and stirred for 30 s, and the reaction was carried out for 120 min at 37ºC. Finally, 60 μL of BSTFA reagent was added, and the reaction was carried out for 90 min at 37ºC and 12000 r/min freezing. All samples were analyzed by GC-MS.
GC-MS Analysis
Metabolites were analyzed by GC-MS with reference to the modified method of Lisec et al [15]. The metabolite content was detected using a 7890A GC/5975C MS system, the mass spectral data were analyzed using Chroma TOF software (V 4.3x, LECO) for peak identification, data baseline filtering and integration, and the substances were identified using the LECO-Fiehn Rtx5 database [16].
Data Analysis
Principal component analysis (PCA), loading plot analysis (loading plot), partial least squares analysis (PLS-DA), and orthogonal partial least squares-discriminant analysis (OPLS-DA) were performed after data normalization using SIMCA-P 14.1, t-tests were performed to screen for differential metabolites by SPSS 23, and clustering heat map analysis and metabolic pathway analysis were performed by using the HIPLOT PRO (https://hiplot.com.cn/) and MetaboAnalyst (https://www.metaboanalyst.ca/) platforms for clustering heat map analysis and metabolic pathway analysis.
Results
Effect of Saline-alkali Stress on the Growth of Rice Seedlings
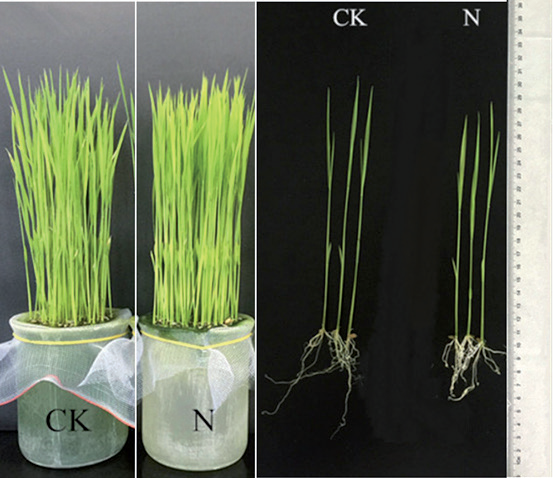
Saline-alkali stress inhibited the growth of rice seedlings (Fig. 1). As shown in Table 1, plant height, root length, dry weight of above-ground and below-ground parts, and relative growth rate of rice seedlings under saline-alkali stress were significantly reduced compared to the control group (P<0.05).
Multivariate Statistical Analysis of Metabolites
This study used PCA and OPLS-DA to analyze all metabolites to determine the factors affecting metabolite differences. According to the PCA scoring plot (Fig. 2), all samples were within the 95% confidence interval, PC1 was 0.395 and PC2 was 0.121, which indicated that there was a significant difference between the two treatment groups, and the results of the five replicates of the data assay were clustered together, which indicated that there was little difference between the replicates and that the data reliability was high. In the OPLS-DA score plot, all the samples under the same treatment were clustered together, indicating that the model responded well to the differences between the two treatments (Fig. 3). Citric acid, oxalic acid, pyroglutamic acid, l-malic acid, sucrose, succinic acid, serine, sedoheptulose, fructose, stearic acid, and other carbohydrates, fatty acids, organic acids, and amino acids were the main components of PC1, and carbohydrates and organic acids, such as 2-deoxy-d-galactose, d-glyceric acid, shikimic acid, and quinic acid were the main PC2 components (Fig. 4).
Quantitative and Qualitative Metabolite Analysis
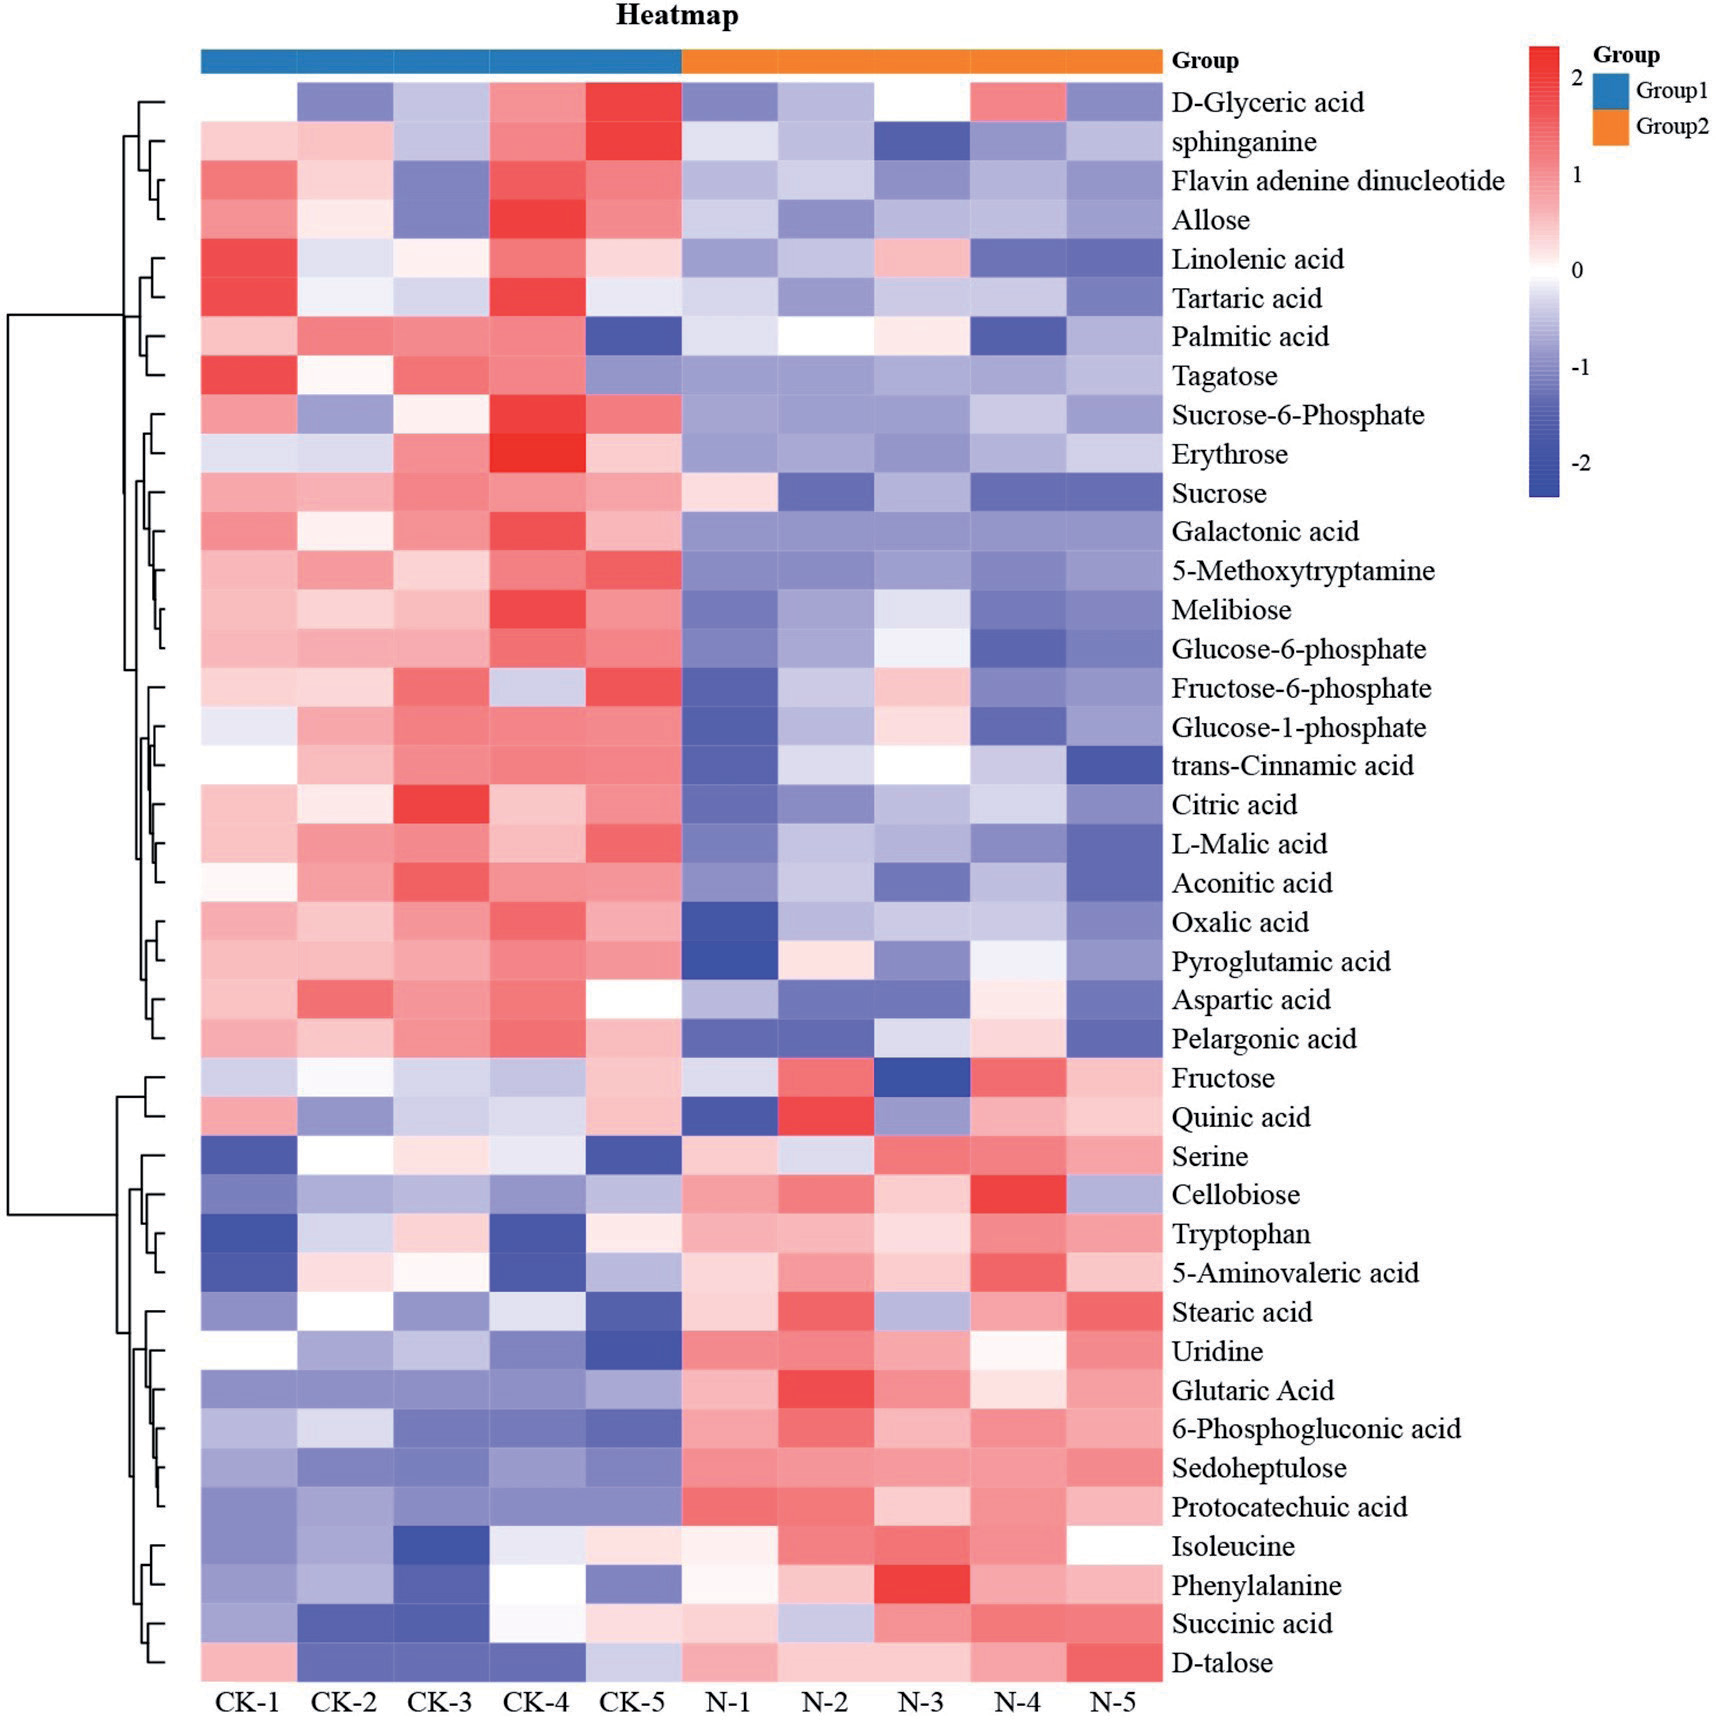
Differential metabolites were screened based on a combination of variable weight values (VIP>1) and t-tests (P<0.05) and the regulation level of metabolites was expressed as log2FC. In this study, a total of 111 metabolites of rice seedlings under saline-alkali stress were identified, including 41 differential metabolites, which were categorized into six major groups (Table 2), mainly including 7 glycolysis and TCA cycle intermediates, 7 amino acids, 11 carbohydrates, 8 organic acids, 4 fatty acids, and 4 other compounds. Fold change analysis showed that 16 metabolites were significantly increased, while 25 metabolites were significantly decreased. Among them, the content of protocatechuic acid was increased most significantly, with a Fold Change value of 5.34. Hierarchical cluster analysis was used to visually display the changes in the levels of differential metabolites between the two treatment groups (Fig. 5).
Table 1.
Changes of growth parameters of rice seedlings under saline-alkali stress.
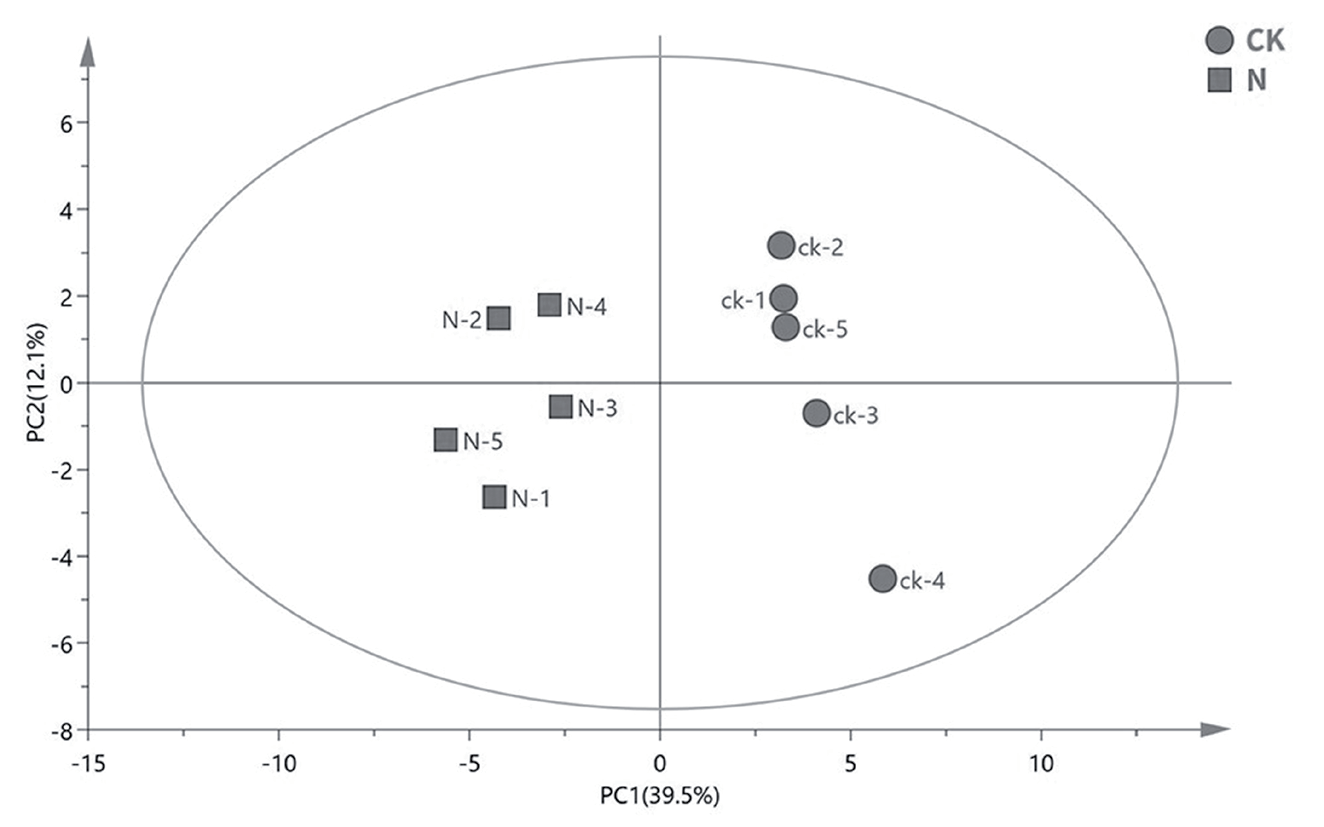
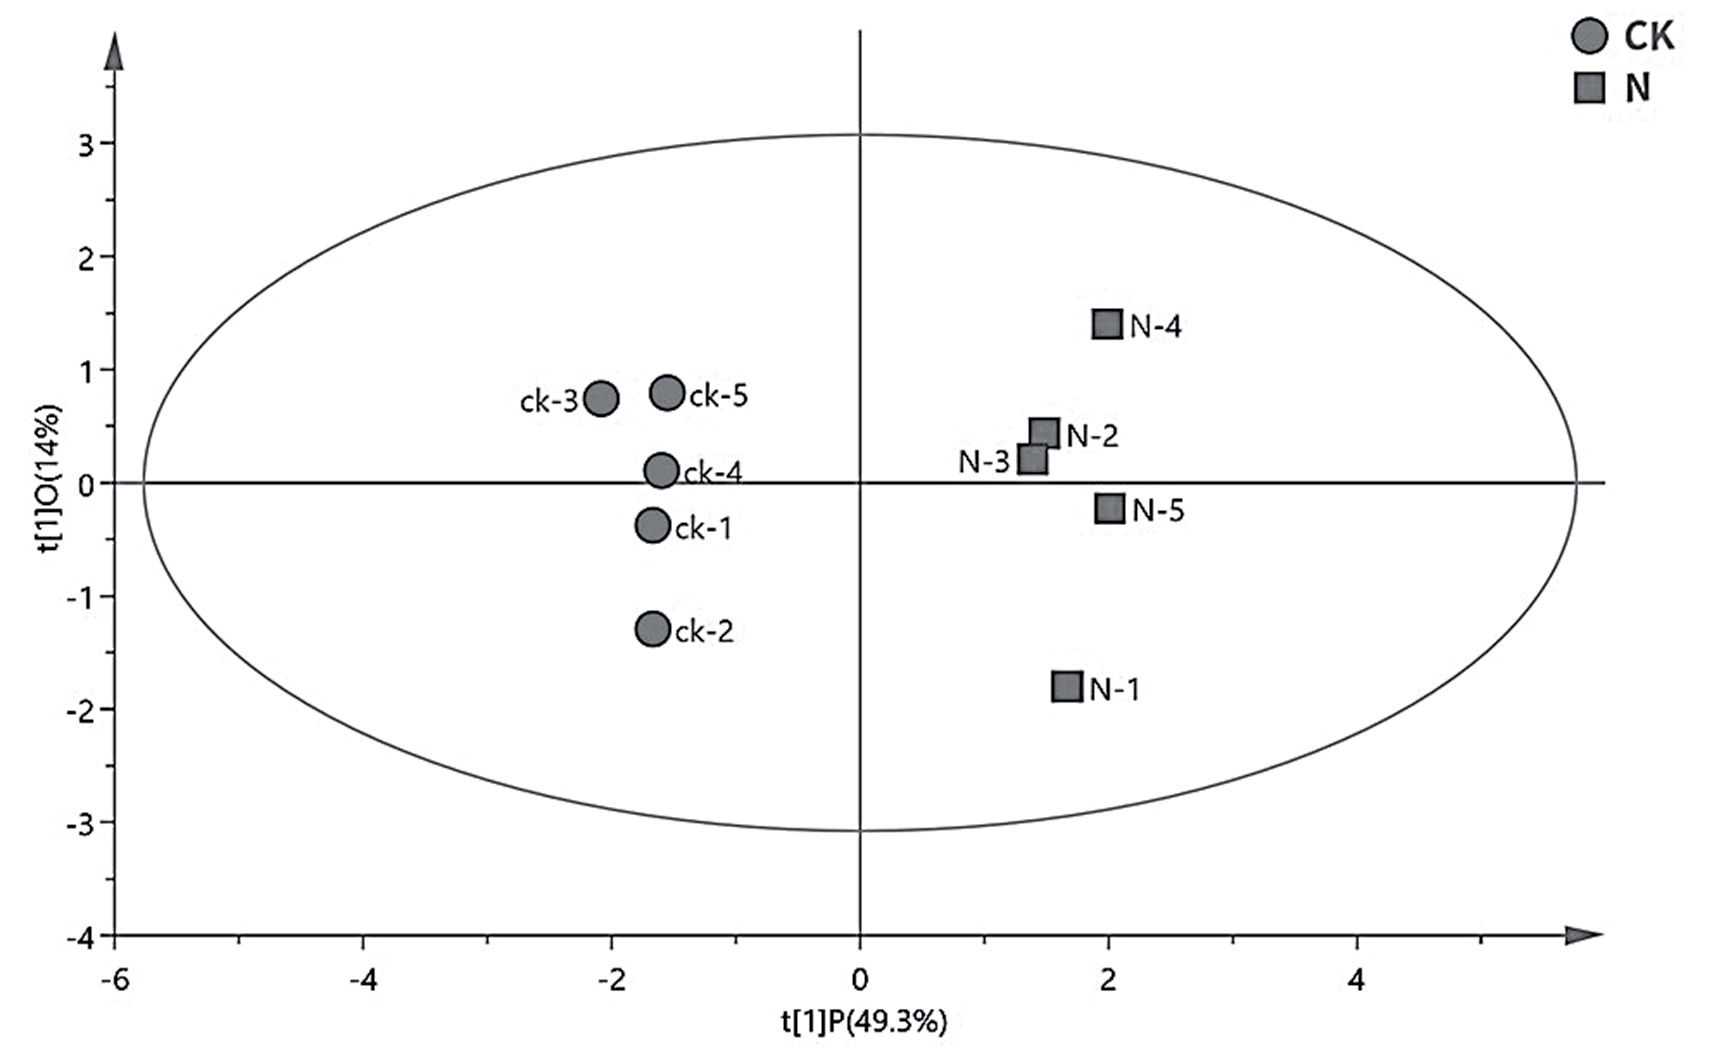
Fig. 4.
The loading of metabolites to the PC1 and PC2. Note: 1: citric acid; 2: oxalic acid; 3: pyroglutamic acid; 4: l-Malic acid; 5: sucrose; 6: succinic acid; 7: serine; 8: sedoheptulose; 9: fructose; 10: stearic acid; 11: 2-deoxy-d-galactose; 12: d-glyceric acid; 13: shikimic acid; 14: quinic acid
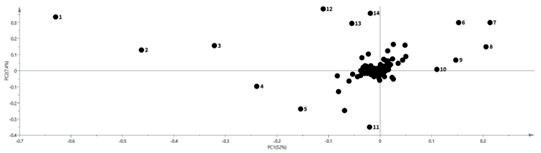
Table 2.
Differential metabolites in rice seedlings under saline-alkali stress.
KEGG Pathway Analysis of Differential Metabolites
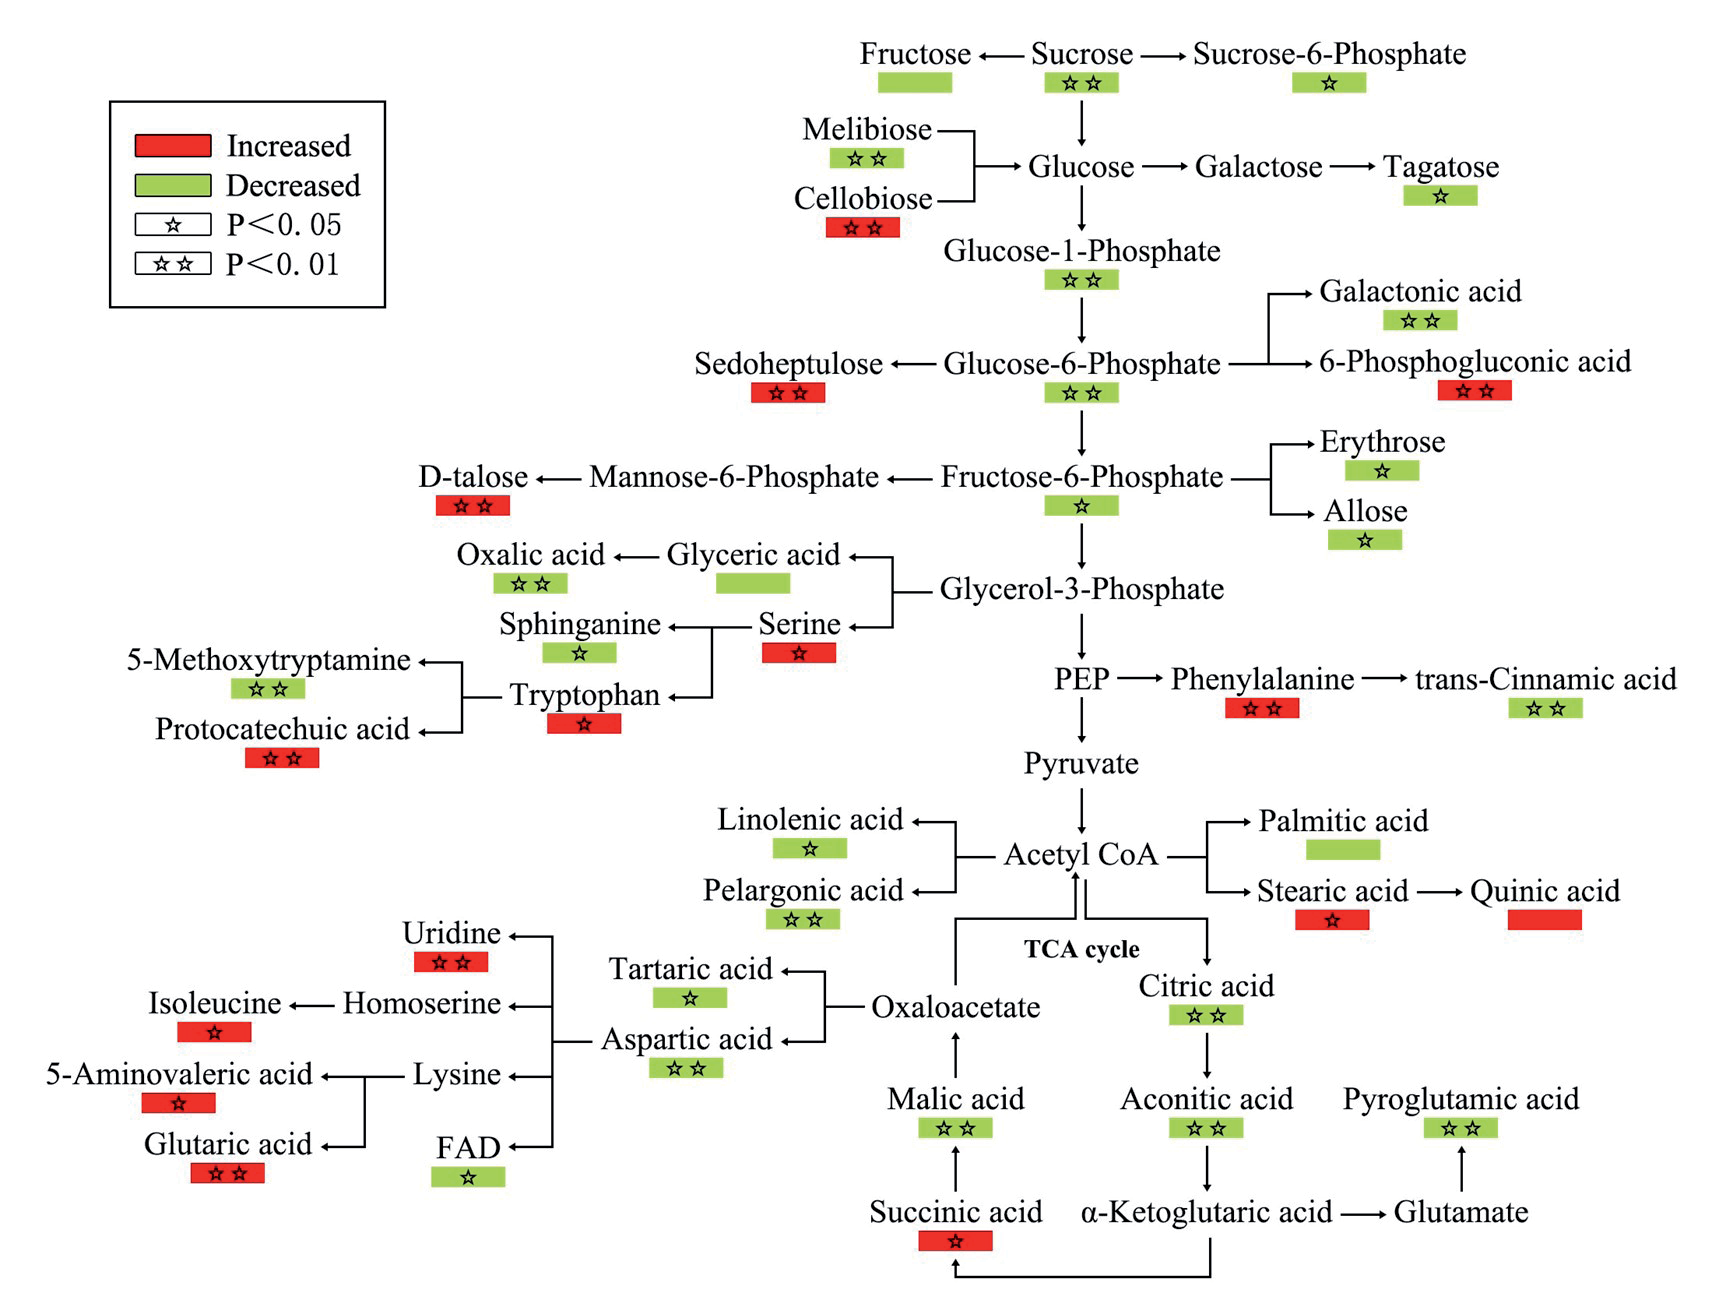
KEGG pathway analysis of rice seedlings under saline-alkali stress can provide a better understanding of differential metabolic pathways. Forty-one differential metabolites were annotated to a total of 36 metabolic pathways, including starch and sucrose metabolism, glyoxylate and dicarboxylic metabolism, TCA cycle, alanine, aspartate and glutamate metabolism, pentose phosphate pathway, etc. (Fig. 6, Table 3). Plants usually regulate physiological metabolic pathways to adapt to stress environment. Compared to CK, obvious differences of metabolites levels in metabolic pathways of saline-alkali stressed rice seedling were shown in Fig. 7.
Discussion
Saline-alkali stress disrupted the ionic balance of plants, leading to ionic stress and osmotic stress. This disruption inhibits growth, synthesis of osmoregulatory substances, and lipid metabolism processes, ultimately reducing plant biomass and affecting yields [17]. Ling et al. [18] observed that salt-stressed rice exhibited yellowing of leaves, reduction in plant height, and decrease in dry matter accumulation. Lv et al. [19] also found that saline-alkali stress resulted in varying degrees of reduction in root length, root surface area, root volume, etc. in rice seedlings. In this study, we discovered that saline-alkali stress significantly reduced plant height, root length, biomass, and relative growth rate of rice seedlings. Additionally, the leaves turned yellow, indicating an inhibitory effect of saline-alkali stress on the growth of rice seedlings.
Stress tolerance is a specific physiological and biochemical process of plant growth and development. Currently, there is limited knowledge about salt tolerance, including osmoregulation, ion transport, and antioxidant protection [20]. To adapt to the osmotic balance between the cytoplasm and the environment, plants accumulate low-molecular-weight metabolites, called compatible solutes, that help reduce the water potential in the cytoplasm [21]. These compatible solutes mainly include carbohydrates, amino acids, and organic acids [22]. Carbohydrates mainly come from the pathways of photosynthesis, glycolysis, and polysaccharide degradation, making them the most important energy substances for plant life activities, and providing plants with a source of energy and a carbon skeleton [23]. Guo et al. [24] found that the carbohydrate content of wheat root decreased significantly under alkali stress. In the present study, we also found a significant decrease in carbohydrate content under saline-alkali stress. Starch and sucrose metabolism mainly involves two parts: the breakdown of sucrose into glucose and fructose, and the synthesis of starch. On the one hand, it can provide raw materials for the TCA cycle and amino acid metabolism, and on the other hand, it synthesizes starch to store energy [25]. Pathway analysis showed that all the differential metabolites related to starch and sucrose metabolic pathways were down-regulated, and sucrose content was significantly reduced. This indicates that saline-alkali stress reduces the photosynthetic rate and inhibits carbon metabolism in rice seedlings, which inhibits starch and sucrose metabolic pathways. Our previous study indeed showed the damage of photosystem (PS) II [26] and a significant decrease in photosynthetic rate [13] due to the accumulation of Na+ in the cells of rice seedlings under saline-alkali stress [14], which ultimately led to a decrease in carbohydrate content.
Fig. 6.
Metabolic pathways in rice seedlings under saline-alkali stress. Note: The X-axis indicates the degree of KEGG enrichment of the substance, the Y-axis indicates the KEGG pathway of enrichment, the color on the right side indicates the P-value of the hypergeometric distribution test for KEGG enrichment, and the size of the circle indicates the amount of enriched substance.
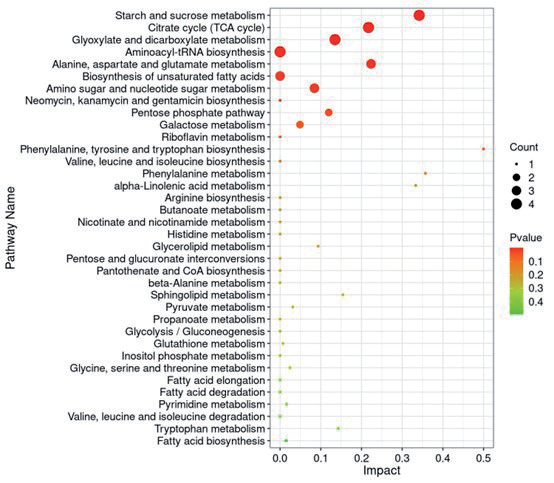
Table 3.
Analysis of key metabolic pathways.
[i] Note: Pathway: Metabolic pathway name; Total: Quantity of metabolites in metabolic pathways; Hits: Number of pathways in differential metabolites; Raw p: P-values for pathway enrichment analysis; −ln(P): P-values are negative logarithms with e as the base; Holm adjust: P-values corrected for multiple hypothesis testing by the Holm-Bonferroni method; FDR: P-values corrected for multiple hypothesis testing by the false discovery rate methodology; Impact: Impact values for topology analysis; Hits Cpd: KEGG ID of differential metabolites.
Fig. 7.
Changes in differential metabolites of metabolic pathways in rice seedlings under saline-alkali stress.
Amino acids are the basic units that make up proteins and play an important role in maintaining intracellular osmotic regulation, the structural integrity of proteins, and the in-plant response to stress [27, 28]. Urano et al. [29] found that the amino acid content in leaves of Arabidopsis thaliana increased significantly under osmotic stress. We also found that amino acid metabolites increased significantly in rice seedlings under saline-alkali stress, presumably due to the degradation of proteins into amino acids, which maintained cellular osmotic homeostasis and/or were involved in the TCA cycle for energy production. Alanine, aspartate, and glutamate metabolism processes are associated with plant growth and development, hormone regulation, and stress resistance responses [30], which decreased in rice seedlings under saline-alkali stress, may be attributed to the uninterrupted nitrogen supply that helps in maintaining optimum plant growth at the control level, even in the stress condition. Overall, amino acid metabolism is closely related to energy and carbohydrate metabolism, carbon and nitrogen balance, protein synthesis, and secondary metabolic requirements [31]. Organic acids, as osmotic regulators, play a key role in maintaining water balance, regulating osmotic pressure, tolerating environmental stress, and forming precursors for amino acid biosynthesis [32]. Sun et al. [33] showed that Cd stress significantly inhibited the secretion of partial organic acids in the roots of S. plumbizincicola. In this study, except for glutaric acid and protocatechuic acid, most of the organic acids were down-regulated.
The respiratory pathways are central to the production of a variety of plant metabolites, including amino acids, lipids, and related compounds, etc [34]. The intermediates of TCA cycle play a crucial role as the starting point for numerous biosynthetic pathways [35]. This cycle of self-regulation allows plants to accumulate or degrade specific small molecules, adapting to the environment, and maintaining internal environmental homeostasis. [36, 37]. Guo et al. [38] found that drought stress significantly reduced malic, citric, and aconitic acids in wheat leaves. We also found that the contents of malic acid, aconitic acid, and citric acid decreased significantly in rice seedlings under saline-alkali stress, indicating that various metabolic equilibria were disrupted when rice seedlings were subjected to stress, and the TCA cycle was inhibited. The pentose phosphate pathway (PPP) is an important pathway of respiratory metabolism in plants that produces NADPH for reductive biosynthesis [39]. Pathway analysis showed a significant accumulation of 6-phosphogluconic acid, a key metabolite of PPP. This indicated that rice seedlings can produce more reducing power through the PPP under saline-alkali stress.
Fatty acids are the main components of cell membrane lipids [40]. β-oxidation is the main way of decomposing fatty acids and can provide a large amount of energy required for life activities. Therefore, it plays an important role in plant growth and development stages and in regulating stress responses [41]. Lu et al. [20] found that the fatty acid content of wild soybeans decreased under salt stress compared with cultivated soybeans. In the present study, we found that the fatty acid content of rice seedlings, except stearic acid, decreased under saline-alkali stress. Glyoxylate and dicarboxylic metabolism provide energy to the organism, promote plant growth and development, and play an important role in plant stress tolerance [42]. The pathway analysis showed that the contents of differential metabolites related to both glyoxylate and dicarboxylic acid metabolism were reduced in rice seedlings, indicating that saline-alkali stress significantly inhibited the metabolism of glyoxylate and dicarboxylic acid, which limited the growth and development of rice seedlings.
Among these metabolites, protocatechuic acid is the most abundant differential metabolite. In the control group, no protocatechuic acid content was detected. Protocatechuic acid is a phenolic acid and a natural antioxidant that plays an important role in clearing oxidative stress and preventing oxidative damage [43]. Thammapat et al. [44] found that protocatechuic acid content was significantly increased in glutinous rice under salt stress, which is consistent with our results.
Conclusions
In this study, we analyzed the changes of differential metabolites in rice seedlings under saline-alkali stress. We identified 41 differential metabolites (16 up-regulated and 25 down-regulated), among which 11 differential metabolites significantly affected five important metabolic pathways, including starch and sucrose metabolism, glyoxylate and dicarboxylic metabolism, TCA cycle, alanine, aspartate and glutamate metabolism, and the pentose phosphate pathway. These results provide a new perspective on understanding the metabolite composition and differences of rice seedlings under saline-alkali stress and lay the foundation for in-depth research on the metabolic mechanism of rice seedlings in response to saline-alkali stress.

