

Introduction
Leptochloa chinensis L. commonly called red sprangletop. It is a grassy weed belonging to the family Poaceae. Its physiological characteristics classify it to be a C4 plant [1]. It is native to tropical Asia and widely distributed in South and Southeast Asia, Australia, and Africa. Geographically, it is distributed in China, Korea, Japan, Bangladesh, Philippines, Pakistan, Cambodia, India, Malaysia, Myanmar, Sri Lanka, Vietnam and Thailand [2]. It is summer annual or perennial tufted grass that can attain up to 120 cm height, having hollow, cylindrical, erect stems, and linear smooth 10-30 cm long leaves. Inflorescence is a narrowly ovate, loose panicle with two rows of 2-3 mm long spikelets that are purplish or green and 4-6 flowered. It reproduces both sexually and asexually [3]. Leptochloa chinensis is known to be an invasive weed in Southeast Asia [4]. It has abundant seed-producing ability, thus widespread in almost all crops including rice. The other characteristics that make it a successful invasive weed are strong allelopathicity, adaptability to variable soil conditions, and aggressive growth habits. Two plants of L. chinensis cause a 55% yield reduction in rice [5]. Due to its hydrophytic nature and amphibious adaptation, it can thrive best under alternate soil flooding conditions. It has dominated all the weeds of rice [6, 7]. That is why; it has now become a serious weed of transplanted as well as direct-seeded rice.
In Pakistan, rice is mostly cultivated through transplanting the nursery-grown seedlings to flooded field conditions. However, to save labor and time, farmers are widely adopting direct seeding technology in which rice seed is directly sown in dry soil conditions. This shift from traditional transplanting to direct seeding has resulted in a change in weed flora [8, 9]. The weeds that were previously considered minor weeds have now become major weeds. L. chinensis is also one of the examples of a dominant weed in direct-seeded rice (DSR). The importance of this weed has increased due to the fact that contrary to other DSR weeds, L. chinensis is very difficult to control even by the use of all existing herbicides [10, 11]. To launch a successful management program against a weed, knowledge of its germination ecology is of utmost importance. Seed germination is affected by a number of factors (Fig. 1) including soil pH, temperature, seeding depth, water ponding conditions, and soil salinity [12]. Soil pH has a minute role in germination, yet it affects the germination process by mediating the availability of nutrients. Temperature is directly linked with the germination process, thus considered the major environmental factor affecting seed germination [13, 14]. Sowing depth also influences the germination and seedling emergence by mediating the supply of light, moisture, and temperature to germinating seed. Water ponding conditions in the seed germination medium reduce germination by restricting the supply of O2 to germinating seed [15]. Salinity inhibits germination by imposing osmotic effects and ionic effects on germinating seed. However, the effect of salinity varies according to plant species, genotypes and environmental conditions. Salinity adversely affects the germination and growth process through its osmotic effect by retarding the imbibition process and its specific ionic effect by imposing toxicity of undesirable ions. The lowering of the osmotic potential of the germination medium imposes a more dominant influence on germination compared with specific ion effects. The seedling growth is mostly suppressed due to specific ionic stress, depending on the amount and distribution of rainfall [16, 17]. The disastrous influences of salt stress are altered by intermingling with other environmental attributes like temperature and light. The ecological optima of germination and early seedling growth of an invasive weed species determines its chances of success in a new region. Therefore, knowledge about the ecology of the germination of a weed can act as a tool for its better management [18].
The allelopathic effect of red sprangletop on rice and the effect of different agronomic practices on its growth in rice have been widely studied. However, very little research has yet been done on the germination ecology (temperature, salinity, pH, burial depth and ponding conditions) of L. chinensis [19]. Knowledge about the optimum and sub-optimum levels of all these environmental factors on germination of L. chinensis can contribute to the development of an effective management program for this weed in direct-seeded rice. A study was therefore being planned to investigate the ecology of L. chinensis so that facts could be established about how it has flourished very much in direct-seeded rice conditions in Pakistan [20].
Materials and Methods
To know about the effect of pH, salinity, temperature, seed burial depth and water ponding conditions on the germination of L. chinensis, 5 individual experiments were carried out, respectively. In experiment 1, treatments consisted of six variable pHs ranging from 5 to 10. The pH of different buffer solutions was maintained by using hydrochloric acid (HCL) and sodium hydro-oxide (NaOH) with MES, HEPES, and tricine were used as buffers. In experiment 2, treatments comprised of 6 increasing salinity levels maintained by variable NaCl solution concentrations viz. 0 (Distilled water), 50 mM, 100 mM, 150 mM, 200 mM, 250 mM and 300 mM. Different levels of salinity were generated by using sodium chloride (NaCl) solution. In experiment 3, treatments were six variable temperatures viz. 20oC, 25oC, 30oC, 35oC, 40oC and 45oC. The experiment 4 comprised of 7 different burial depths viz., 0 cm (on surface of soil), 1 cm, 2 cm, 3 cm, 4 cm, 5 cm and 6 cm. In 5th experiment, different ponding conditions viz. 0 cm, 2 cm, 3 cm, 4 cm, 5 cm, and 6 cm were maintained as experimental treatments. In the first three experiments, 25 seeds of L. chinensis were spread in a petri plate (9 cm in diameter) with having double layer of filter papers. In the pH experiment, 5 ml buffer solutions of different pH levels, in the salinity experiment, 5 ml of solutions with different salinity levels, whereas in the temperature experiment, 5 ml of distilled water were applied to petri plates and petri plates were enclosed with parafilm to avoid moisture loss. Petri plates in the first two experiments were put into the germinator at 35oC while in the third experiment, at different temperatures as per the treatment plan. In the fourth and fifth experiments, 25 seeds of L. chinensis were sown in pots (9 cm diameter) filled with soil. In sowing depth experiment, seeds of L. chinensis were sown in soil saturated with distilled water at a prescribed depth according to the treatment plan and then pots were irrigated with distilled water as per requirement. However, in the water ponding experiment, seeds of L. chinensis were sown on the surface of the soil and then pots were irrigated with distilled water to maintain the proposed ponding conditions throughout the study as per the treatment plan. Pots were kept in the germinator at 35oC temperature. The germination/emergence data were collected on a daily basis for the period of 20 days. The seed was supposed to be germinated when radicle and plumule attained 2 mm length and the sprouted seed was poured out of the petri dish / pot after counting. Soil used in pots was collected from the site without any vegetation at Agronomic research farm. Collected soil was sieved and then filled in plastic pots.
Following parameter was recorded in all experiments:
1. Germination /emergence percentage (GP/EP)
Based upon final germination / emergence count, germination / emergence percentage was calculated according to formula of The Association of Official Seed Analysts [21].
2. Time to start germination / emergence (Ti)
It is the time in days when seeds start germinating / emerging.
3. Germination/emergence index (GI/EI)
The Germination Index was determined as portrayed by the Association of Official Seed Analysts, (1990) by the following Equation (2):
(2)
4. Mean germination/emergence time (MGT/MET)
Mean germination/emergence time was determined by the situation of [22].
Where n = Number of seeds that had germinated on day “D” D = Number of days counted from the beginning of germination.
5. Time to 50% germination/emergence (T50)
The time to obtain 50% germination/emergence (T50) was determined by the equation of [23] as adjusted by [24]
Where N = Last number of germinated / emerged seeds ni & nj = Accumulative number of seeds germinated by contiguous counts at times ti and tj, individually, where ni <N/2 < nj.
6. Seedling vigor index (SVI)
Germination percentage and seedling length were used to calculate seedling vigor index (SVI) by the succeeding method as designated by [25]
Statistical Analysis
All the experiments were arranged as completely randomized designs with each treatment having four replications. All the experiments were repeated twice. Data were subjected to a one-way analysis of variance (ANOVA) and all possible comparisons among treatment means were made through the least significant difference test. Germination percentage data in response to increasing NaCl concentrations, sowing depths and flooding depth were fitted to a functional three-parameter logistic model using Sigma Plot 2008 (Version 11.0, SyStat Software GmbH, Schimmelbuschstrasse 25 D-40699 Erkrath Germany). The model equation fitted for NaCl concentration experiment was:
Where G is the total germination at x NaCl concentration, x50 is the NaCl concentration for 50% inhibition of the maximum germination and g indicates the slope. The model equation fitted for sowing and flooding depths experiments was:
Where E is the total emergence at x sowing and flooding depth, x50 is the sowing and flooding depth for 50% inhibition of the maximum emergence and e indicates the slope.
Results and Discussion
Effect of pH
The pH value expresses the acidity or alkalinity of the solution on a logarithmic scale. Germination of L. chinensis was significantly influenced at various pH levels (Fig. 2, Table 1). The pHs 6 and 7 attained the highest germination percentages (77 and 78%, respectively) (Fig. 2). The earliest time to germination initiation (Ti) (3.75 days) was recorded with a pH 8 (Table 1). The maximum germination index (19.54) was recorded with Petri plates that were supplied with a solution having pH 9 which was statistically similar to pH 8 (Table 1). The maximum germination speed of L. chinensis seeds was observed with pH 8 as the lowest values of MGT (5.09 days) and T50 (5.63 days) were noted with it. However, pH 9 also gave significant at par values of MGT and T50.
The better germination performance of L. chinensis seeds at slightly acidic to alkaline pHs seems to be the result of enhanced activity of enzymes involved in the germination process enzymes are directly affected by the H+ ion concentration in the germination medium. Our outcomes are in accordance with the outcomes of [26] who described that pH may not be a restricting component for the emergence of turnip weed. Correspondingly, higher than 45% emergence was observed over a pH range from 4-10. [27] described that germination of seed was pragmatic over a broad range of pH however maximum germination percentage of L. chinensis was recorded at pH 7 while E. glabrescens was proved to be more sensitive to given range of pH. Our consequences are also in agreement with the observations of [28] who observed that the highest germination of L. fusca (92%) was recorded at pH 7 while the lowest value of germination (54%) was observed at pH 10.
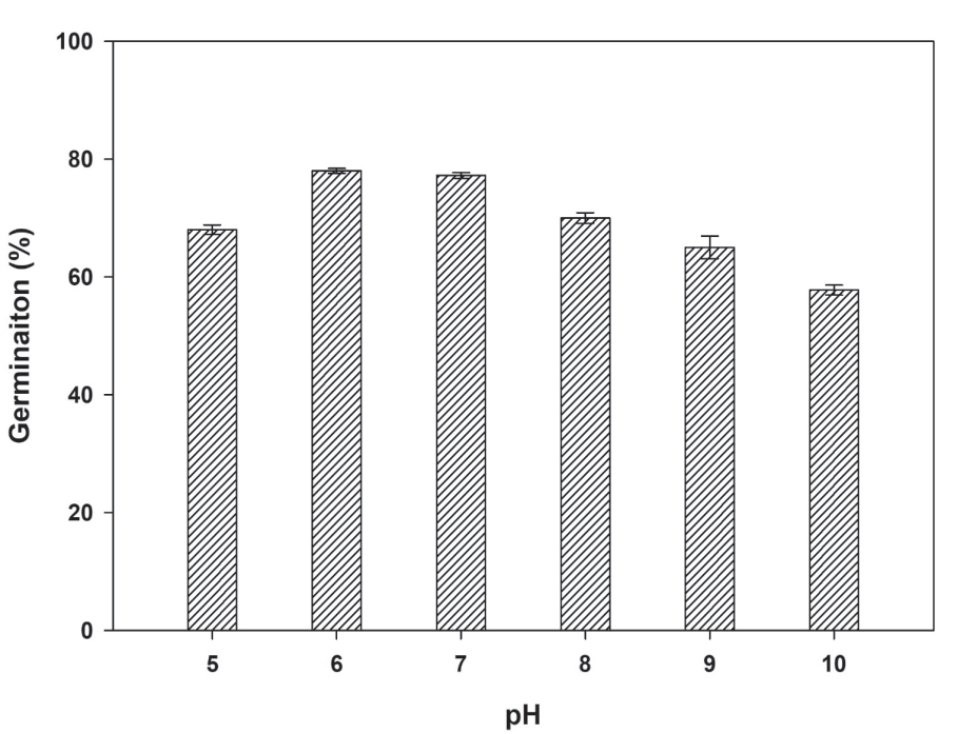
Table 1.
Influence of variable pHs, salinity levels and temperatures on germination of Leptochloa chinensis L.
Effect of Salt Stress
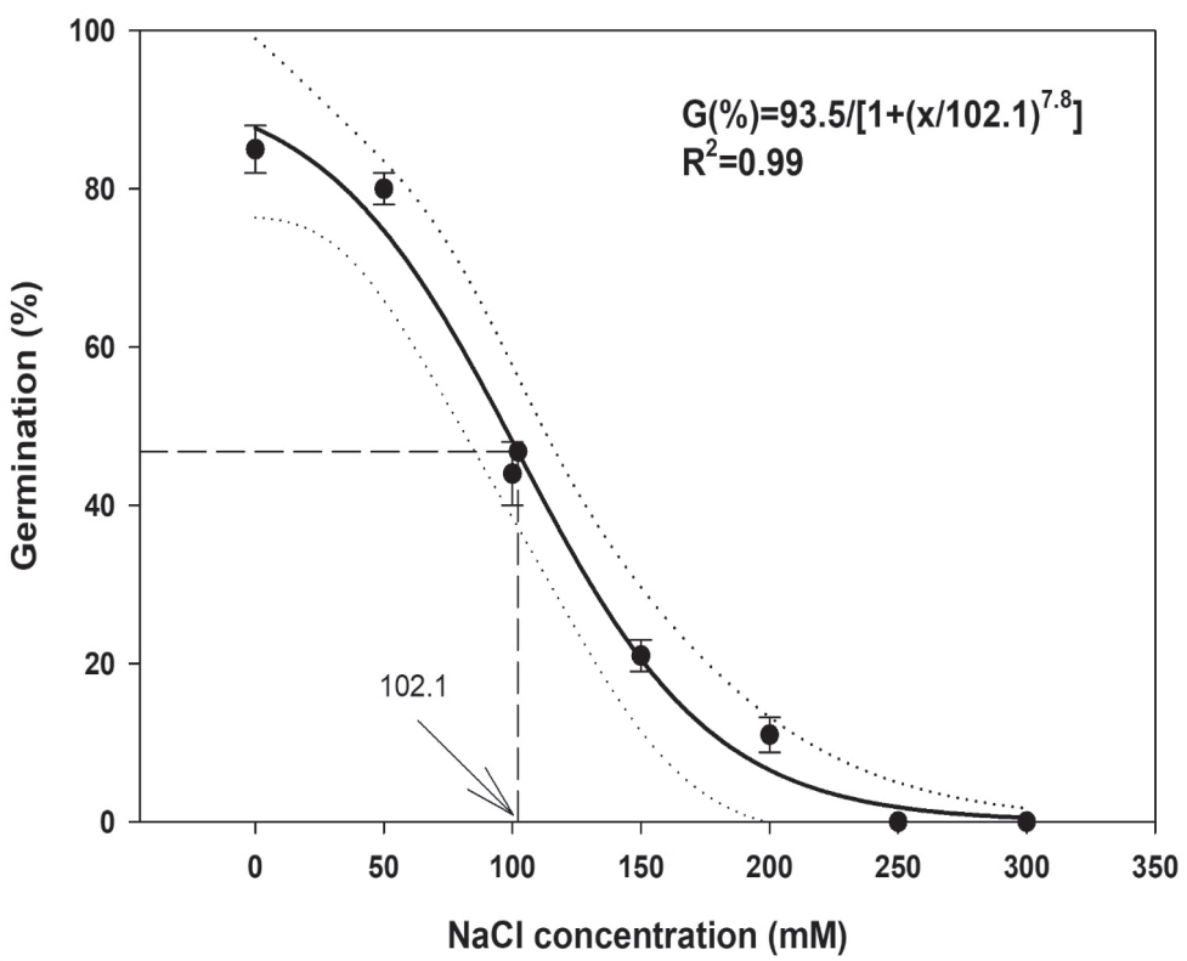
The term salinity refers to the quantity of dissolved salts that are present in water. Data given in Table 1 indicated that different levels of salinity significantly reduced the germination of L. chinensis. Results revealed that germination of L. chinensis was significantly reduced by the increase in NaCl concentration from 0 to 200 mM whereas no L. chinensis seed germinated beyond 200 mM NaCl concentration. According to the 3-parameters logistic model estimation, 50% germination of the maximum germination of L. chinensis occurred at 102 mM NaCl concentration (Fig. 3). The earliest germination initiation (4.25 days) and T50 (6.62 days) of L. chinensis occurred at 0 mM NaCl concentration that was not significantly delayed up to 50 mM NaCl concentration beyond which these were significantly increased (Table 1). The GI and MGT of L. chinensis followed the same trend as the highest value of GI (20.6) and the lowest value of MGT (6.06 days) were recorded with control. However, a significant delay in germination in terms of these parameters occurred at and beyond 50 mM NaCl concentration. Higher soil saltiness hinders seed germination because of the low osmotic potential of water created around the seed, which hinders water imbibition by seed [29]. Moreover, a higher concentration of Na and Cl in the germination medium might itself prove poisonous to seeds [30].
Fig. 3.
Effect of NaCl concentration on germination (%) of L. chinensis. The bold line represents a three-parameter logistic model (G (%) = Gmax/[ 1 + (x/x50)g]) fitted to the data. The vertical dashed line represents X-axis value at 50% of the maximum germination. The dotted lines show 95% confidence intervals. Vertical bars represent±standard error of the mean.
Plant emergence and growth are significantly hampered in saline soil owing to peripheral osmotic potential to avert water uptake or the poisonous effect of sodium and chlorine on germinated seed [31]. These outcomes are similar to the observations of [32] who pointed out that germination of E. colona was reduced linearly by the escalation in NaCl concentration. The germination of barnyard grass was substantially reduced due to the influence of salinity. Present findings are also similar to those of [33] who documented that the germination index was linearly decreased by the increase in NaCl concentration. Our observations are also in accordance with those of [34] who documented that MGT was increased with the increase in salt concentrations. At high levels of salinity, seeds of different weeds significantly delayed their 50% germination.
Effect of Temperature
The data regarding germination of L. chinensis at different temperatures indicated that germination of L. chinensis was significantly influenced at various temperature regimes (Fig, 4, Table 1). Significantly, the highest germination percentage (92%) was noted at 35oC temperature (Fig. 3). The germination by L. chinensis seeds was started earlier (4 to 6 days) within the temperature range of 20oC to 40oC, while the temperature above 40oC significantly delayed it. The earliest germination completion in terms of T50 (6 to 7 days) and MGT (7.50 to 7.72 days) of L. chinensis occurred within 20oC to 25oC temperature range. However, the overall germination speed of L. chinensis was the highest at 25oC to 40oC as indicated by the highest values of GI (13.6 to 15) recorded within this temperature range.
Germination of L. chinensis was better at moderate to high temperatures. This is because this weed is native to tropical regions characterized by high temperatures. Similar results were also found by [35] who described that maximum germination of L. chinensis (95%) was recorded at a temperature range from 25-35 oC, indicating high-temperature requisite for germination of red sprangletop. The judgments of the present experiment are alike with the observation of [28] who indicated that germination of E. glabrescens, L. chinensis, and D. aegyptiumwas started at 35oC. However, contrasted results were described by [36] who pointed out that emergence of L. chinensis were non-significant at various temperature regimes. Similarly, the temperature requirement of L. chinensis was even higher than those of other aquatic weed species, as reported by [37].
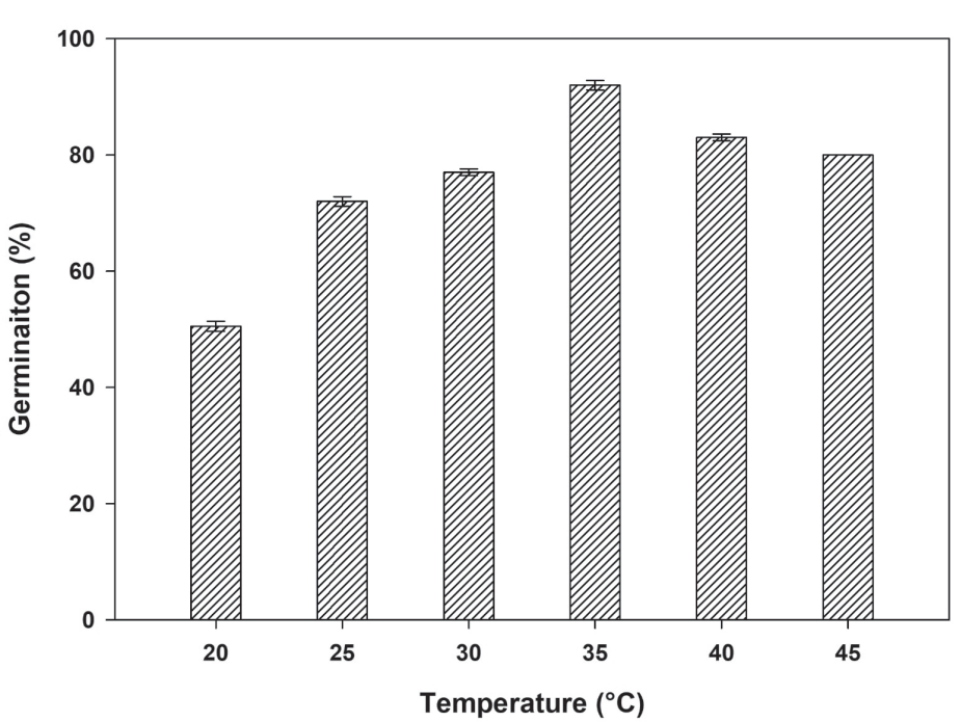
Table 2.
Influence of variable burial depths and ponding conditions in germination of Leptochloa chinensis L.
Effect of Burial Depth
Data related to the effect of different burial depths in soil on the emergence of L. chinensis seed have been given in Table 2. Results indicated that the emergence of L. chinensis seed was significantly reduced as its sowing depth was increased from 1 to 5 cm beyond which no seed could emerge. The fitted model estimated that 50% emergence of the maximum was obtained at 1.56 cm burial depth (Fig. 5). The earliest start of emergence (at 4.25th to 5th day of sowing) of its seeds was observed at 1 to 3 cm burial depth (Table 2). However, a sowing depth of 1 cm attained the highest emergence index (EI) (21.5), the least time to 50% emergence (T50) (5.92 days), and mean emergence time (MET) (6.6 days). However, sowing of L. chinensis seeds below this depth resulted in a significant decline in EI and a delay in T50 and MET.
The L. chinensis showed better emergence at shallower sowing depths because it has minute seeds. Small-seeded weed species may have an insufficient amount of food reserves to support seedling emergence at deeper depths. As the seed goes from shallower to deeper sowing, the light incidence to it is gradually reduced [38]. Our findings are in conformity with those of [39] who documented that no seedling of L. chinensis emerged from a burial depth of 0.5 cm or more. Obtained findings are comparable with the outcomes of [40] who described that sowing depth caused an expansion in MET which rose from 2.5 days in the case of surface sowing (1 cm) to 7 days in the case of deep sowing. Generally, germination of L. chinensis gradually was reduced with the increase in each cm of burial depth. [41] stated that seeds sown under 2 mm depth usually received a restricted extent of light, which isn’t sufficient to start germination of seed. At deeper depths, small-sized seeds, hypoxia, and low gaseous diffusion are also responsible for zero germination. A sowing depth of a few centimeters is adequate to avert emergence, encouraging the typical scalar emergence and emergence regularly present in disturbed habitats [42]. Germination of different weed species gradually decreased by the increase in sowing depth [43]. The maximum emergence of 69% was noted from the seeds planted on the surface or near the surface and no seedlings rose up out of seeds covered at profundities of 0.5 cm or more [44].
Effect of Flooding Depth
Data regarding the germination of L. chinensis as affected by the varying flooding depths have been presented in Table 2. The results reveal that a gradual decline in the emergence of L. chinensis seed occurred as water flooding depth was increased from 0 to 4 cm. However, no L. chinensis emerged out of the soil as the flooding depth was increased beyond 4 cm. A 3-parameters logistic model was fitted to the germination data obtained under different flooding depth (Fig. 6). The model estimated that 50% of the maximum germination occurred at flooding depth of 2.2 cm. The quickest emergence initiation (at 4.25 to 5th day of sowing) of this weed occurred at 0 to 2 cm flooding depth. However, L. chinensis seeds attained the highest EI (19.9), the earliest T50 (6.28 days), and MET (6.74 days) under zero flooded conditions. While flooding caused a significant decline in these parameters that undergo through further decline as flooding depth was increased.
Fig. 5.
Effect of seed burial depth on emergence (%) of L. chinensis. The bold line represents a three-parameter logistic model (G (%) = Gmax/[ 1 + (x/x50)g]) fitted to the data. The vertical dash line represents X-axis value at 50% of the maximum germination. The dotted lines show 95% confidence intervals. Vertical bars represent ± standard error of the mean.
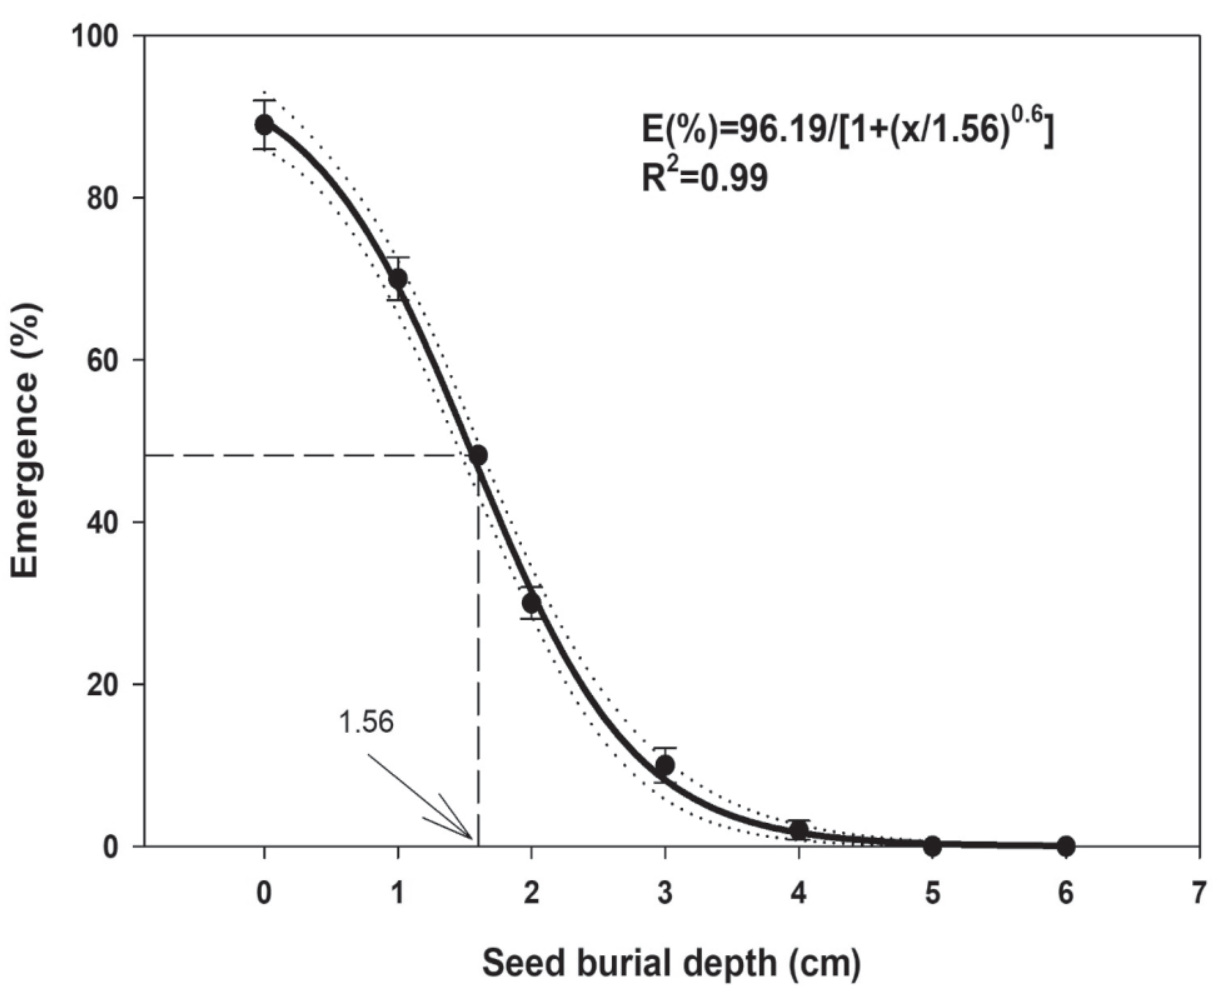
Fig. 6.
Effect of flooding depth on germination (%) of L. chinensis. The bold line represents a three-parameter logistic model (G (%) = Gmax/[ 1 + (x/x50)g]) fitted to the data. The vertical dash line represents X-axis value at 50% of the maximum germination. The dotted lines show 95% confidence intervals. Vertical bars represent ± standard error of the mean.
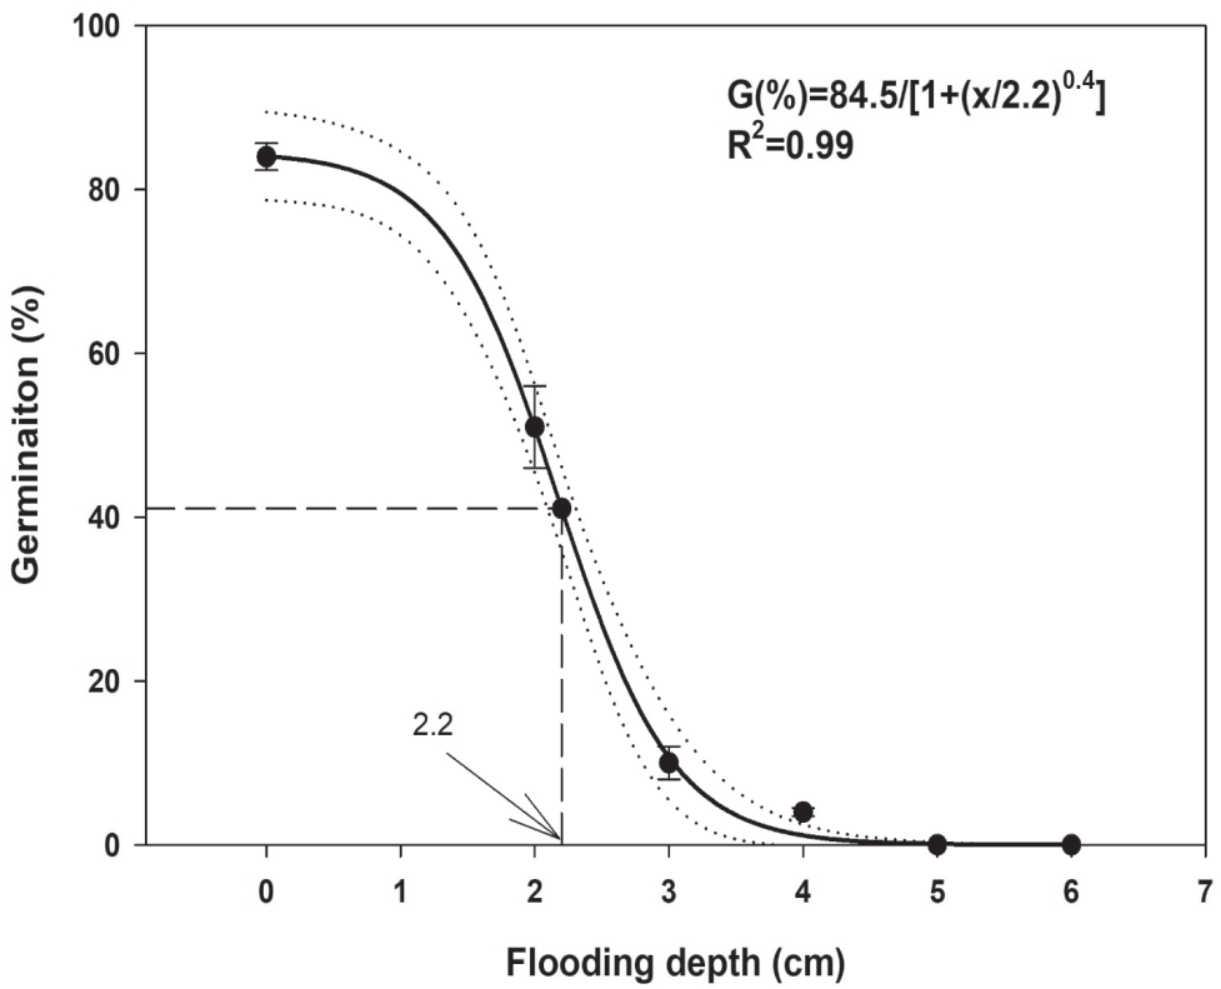
The decline in germination of L. chinensis in response to an increase in flooding depth beyond 2 cm was due to its amphibious nature. Although this weed can grow under flooded rice conditions, yet degree of its infestation in rice increased many folds as farmers shifted from puddled to dry-seeded rice. These outcomes are according to the conclusions of [45] who noted that flooding conditions significantly reduced the emergence and dry matter of red sprangletop. These outcomes also corroborate the observations of [46] who stated that Texas weed seed did not grow under immersed or flooded conditions, yet the seed endured flooding and sprouted (23 to 25%) after flood evacuation.

