

Introduction
Rice is a crucial staple food for a significant portion of the global population. To enhance rice productivity and ensure food security, it is essential to explore the utilization of marginal lands, particularly large saline areas where current elite cultivars exhibit lower yields [1]. There are several biotic and abiotic stress factors that meaningfully affect the growth and yield of economic plants, like drought [2-4] and salinity [5-7]. Salinity is a very effective abiotic factor affecting agriculture and sustainability worldwide [8-10]. It causes harmful impacts on all plant organs [11, 12]. Also, salinity poses a significant challenge to rice cultivation, leading to a significant reduction in annual rice yield [13]. Environmental factors, primarily salt and drought, are responsible for over 70% of global crop output losses [14]. Salinity adversely affects rice growth at all developmental stages, with the early seedling stage being particularly susceptible to its impact [15].
Salt stress induces detrimental effects on plants, particularly through membrane damage, leading to lipid peroxidation, increased production of reactive oxygen species (ROS), and the accumulation of malondialdehyde (MDA). To counteract these effects, plants have developed defense mechanisms such as antioxidant enzymes and low-molecular-weight substances including ascorbic acid (AsA), glutathione, and carotenoids. Salt stress affects various metabolic processes in plant cells, resulting in the excessive accumulation of ROS and oxidative damage. Furthermore, salt stress has been reported to decrease photosynthetic efficiency and cause electrolyte leakage, ultimately reducing plant productivity [16]. However, the exogenous application of salicylic acid has shown promise in mitigating the effects of salt stress on plants [17]. When plants encounter stress conditions, they perceive specific stress signals that activate various signaling modules, including signal transducers, transcription factors, and hormones. These signaling components transduce stress signals, leading to the expression of stress-related genes. The products of these genes then participate in diverse physiological and metabolic processes to mitigate the cellular damage induced by the initial stress signals. Transcription factors play a pivotal role as master regulators of gene expression, orchestrating plant responses to environmental stresses. Notably, diverse families of transcription factors, such as ABRE/ ABF, AP2/ERF, bZIP, and MYC/MYB, along with other regulatory proteins, form complex molecular networks underlying abiotic stress tolerance. In response to environmental pressures, plants demonstrate remarkable flexibility in gene expression, involving the production of osmoprotectants like proline and sucrose, as well as the activation of enzymes that scavenge reactive oxygen species to prevent cellular damage. Additionally, heat shock proteins (HSPs) and late embryogenesis-abundant (LEA) proteins contribute to enhancing stress resilience. Furthermore, plants modify membrane lipid composition to improve fluidity and maintain ion homeostasis, while small RNAs also play a role in contributing to stress responses [18]. LEA proteins, traditionally associated with seed desiccation, have emerged as versatile stress protectors, accumulating robustly in response to various stresses such as Abscisic acid (ABA), freezing, salinity, cold, and drought across different plant tissues, indicating a broader cellular defense mechanism beyond seed development. These proteins are categorized into different structural classes, with all photosynthetic organisms possessing the LEA II group, which includes dehydrins. Dehydrins, characterized by the presence of a conserved K-segment rich in lysine near their C terminus, have been implicated in multifaceted roles beyond desiccation tolerance, including membrane stabilization, enzyme cryoprotection, and reactive oxygen species (ROS) scavenging. Notably, the Y-segment of dehydrins has been highlighted as more crucial for protecting against salt and drought stress compared to cold stress [19-21]. Given their potential, this study aimed to isolate and clone the SK2-type dehydrin1 (DHN1) gene from Egyptian sorghum (Sorghum bicolor) and to transform the rice varieties Giza 177 and Giza 178 with the SbDHN1 gene using biolistic transformation techniques. In addition, the expression of the SbDHN1 gene in transgenic rice will be studied, and its effects on rice salinity tolerance will be evaluated. Finally, a bioinformatic analysis will be performed to characterize the SbDHN1 gene and its produced protein.
Materials and Methods
Plant Materials and Stress Conditions of the SbDHN1 Gene
The seeds of Sorghum cultivar R12 and rice cultivars Giza 177 and Giza 178 were generously provided by the Sorghum Department and Rice Department, respectively, at the Field Crops Research Institute, Agricultural Research Center (ARC), Giza, Egypt. The seeds underwent sterilization and germination according to the protocol outlined by Assem et al. [22]. To isolate the SbDHN1 gene, four-day-old sorghum seedlings were transferred to a half-strength MS medium [23] supplemented with 200 mM NaCl for six days under light conditions. Subsequent to the salt stress treatment, these seedlings were utilized for RNA isolation.
Cloning and Sequence Analysis of the SbDHN1Gene
RNA was extracted from sorghum plantlets that had been subjected to salt treatment. The extraction was carried out using the RNeasy Mini Kit (Qiagen, cat. no. 74104, Germany). Subsequently, the SbDHN1 gene was obtained from the synthesized cDNA using the AccessQuick™ RT-PCR System (Promega, cat. no. A1701, USA) through the process of RT-PCR. Specific primers for the SbDHN1 gene were designed using the Primer3 tools (https://primer3.ut.ee/) based on the nucleotide sequences of Sorghum bicolor dehydrin DHN1 (LOC8077913) mRNA, with accession number XM_002439642.2 as provided by the National Centre for Biotechnology Information (NCBI - https://www.ncbi.nlm.nih.gov/nucleotide/).
Furthermore, for cloning, recognition sequences for the EcoRI and BamH1 enzymes were incorporated into the SbDHN1 gene primers. The PCR amplification of SbDHN1 involved a profile consisting of thirty cycles, each comprising denaturation at 94ºC for 30 seconds, annealing at 60ºC for 45 seconds, and extension at 72ºC for one minute. This was followed by a final extension cycle at 72ºC for five minutes. Finally, the SbDHN1 PCR products were purified using the QIAquick gel extraction kit (Qiagen, cat. no. 28704, Germany).
After the PCR amplification, the SbDHN1 fragment was incorporated into the pGEM-T vector (Promega, USA, cat. no. A1360) with the assistance of T4 DNA ligase (Thermo Fisher Scientific, USA, cat. no. EL0011). Subsequently, this recombinant vector was introduced into competent E. coli cells and cultured on selective media containing IPTG/X-gal/ampicillin. Colonies containing the desired recombinant plasmid were identified and verified through sequence analysis carried out by Macrogen Company in Seoul, South Korea. For plant transformation, the pCambia1390-SbDHN1 vector, which carried the SbDHN1 gene, was designed and visualized using SnapGene software. To assess the similarity of the SbDHN1 gene to known sequences, both nucleotide (BLASTn) and protein (BLASTp) similarity searches were conducted on the NCBI website. Furthermore, the SbDHN1 gene sequence was translated into both coding and non-coding RNA sequences, and the functional attributes of the encoded protein were predicted using online tools accessible via the Swiss Bioinformatics Resource Portal (http:// www.expasy.org). To gain insights into the evolutionary relationships and potential functions of the SbDHN1 protein, its full-length amino acid sequence was aligned with homologous sequences from three closely related crop species: Sorghum bicolor, Panicum virgatum, and Zea mays. This alignment was executed using CLC Sequence Viewer version 6.8.1 software developed by CLC Bio ([A/Swww.clcbio.com]).
Construction of the Plant Expression Vector
Following the confirmation of the SbDHN1 gene through sequencing, the recombinant SbDHN1- pGEM-T vector was subjected to cleavage using the restriction enzymes EcoRI and BamH1. The resulting excised SbDHN1 fragment was subsequently inserted into the pCambia1390 plant expression vector. Before this insertion, the pCambia1390 vector had been pre-digested with the same enzymes, EcoRI and BamH1, to ensure compatibility of the ends for directional insertion. This vector was graciously provided by Dr. Ghada Aboelhaba; AGERI, ARC, Giza, Egypt.
Rice Transformation and Regeneration
Surface-sterilized seeds of rice cultivars Giza 177 and Giza 178 were cultured on a callus induction medium (MS medium provided with 2.5 mg/L 2,4-D, 20 g/L sucrose, and 0.7 mg/L L-proline) under dark conditions at 28ºC for three weeks. Before this, seeds were dehusked and treated with 70% ethanol (1 min), followed by 50% commercial Clorox (30 min), followed by thorough rinsing with sterilized distilled water. For particle bombardment, embryogenic calli were chosen as the target tissue. To enhance particle uptake and improve transformation efficiency, these calli were pre-treated with an osmotic solution containing 45 g/L each of sorbitol and mannitol. This treatment commenced 4 hours before bombardment and continued for 16 hours after the bombardment event. Additionally, the plasmid DNA used for transformation was precipitated onto 0.6 µm gold particles following a modified protocol for the Bio-Rad Biolistic PDS- 1000/He Particle Delivery System. For the particle bombardment transformation, a pressure of 1100 psi and one shot per plate were employed. After bombardment, the calli were placed on callus induction medium for a 7-day recovery period in darkness to promote the healing of the transformed cells. This was followed by transferring the calli to a callus medium provided with 50 mg/L hygromycin for selection. Every two weeks, the calli were subcultured onto a fresh selection medium to continuously maintain selection pressure and propagate the transformed lines. Following transformation, the calli were transferred to a shoot induction medium containing MS salts, vitamins, 3 mg/L benzyl adenine (BA), and 1 mg/L 1-naphthaleneacetic acid (NAA) for shoot regeneration. This incubation occurred under controlled conditions of 28ºC temperature and 16 hours of light per day. Once well-developed shoots with visible leaf primordia were formed, they were transferred to half strength MS medium for root development. After successful root establishment, the putatively transgenic plantlets were acclimatized to ex vitro conditions by immersion in Hoagland nutrient solution. Finally, healthy, rooted plantlets were transplanted into individual pots containing a 1:1:1 mixture of peat moss, soil, and sand. These pots were housed in a greenhouse maintained at 28ºC with 16 hours of photoperiod and 50% relative humidity, as described by Moghaieb et al. [24].
PCR, Semi-Quantitative RT-PCR Analysis
Genomic DNA and total RNA were isolated from rice transgenics and untransformed control plants. PCR analysis was carried out in all the T0 transgenics and 5 selected (M1, M4, M10, M15, and M16) T1 lines and 3 (M1, M4, and M10) T2 progeny. RT-PCR analysis was carried out in 3 selected T2 transgenic plants. PCR and RT-PCR analysis were carried out using the SbDHN1 gene-specific primers and PCR conditions as described above. Semi-q real-time-PCR analysis was also carried out in the selected three transgenic lines (T2). Semi-qRT-PCR was performed using the QuantStudio™ 3 (Applied Biosystems) and the SYBR qPCR Premix ExTaq (Takara). A 1-µl sample of a 1:10 dilution of the cDNA and 0.2 µM of the specified primers were added to the final volume of 20 µl (including 19 SYBR Premix Ex Taq [25]. For the normalization of the desired endogenous transcripts, the rice actin was used as a reference control. The relative quantification expression of target genes was calculated with the comparative cycle thersold (Ct) method (Livak and Schmittgen 2001), according to the following equation: ΔCt = (Ct target gene – Ct reference gene) ΔΔCt = ΔCt treatment – Ct control. Then the relative expression ratio was calculated as (R) = 2^-ΔΔCt.
Southern Blot Analysis
Genomic DNA of five selected PCR-positive T0 transgenics along with an untransformed control was digested with BamH1 and Ecor1 in order to detect the stable integration of the SbDHN1 gene in the regenerated transformed plants according to [26]. The digested DNA was electrophoretically separated on a 0.8% agarose gel, transferred to a positively charged nylon membrane (Boehringer Mannheim), and then cross-linked to the membrane by UV irradiation. The coding sequence of the SbDHN1 gene was used as a probe and using a random priming DNA labeling and detection kit (Roche cat. no. 11093657910). The labeled probe was incubated with the membrane at 65ºC for 16-18hr and the hybridization signals were detected by the colorimetric method.
Evaluation of Transgenic Rice under Salt Stress Conditions
To assess the performance of genetically modified rice plants expressing the SbDHN1 gene under salt stress conditions, a study was conducted using T1 progeny from two transformed cultivars, Giza 177 and Giza 178. Non-transgenic plants served as controls. Ten seeds from each transformed line and the control group were surface-sterilized and germinated for seven days in the dark at 28ºC on half strength MS basal medium supplemented with 1% sucrose. Following germination, seedlings were transferred to half strength MS medium provided with 200 mM NaCl, replicating the conditions described by Wang et al. [27]. These experiments were conducted in triplicate under controlled light conditions at 28ºC. After seven days of salt exposure, the response of young seedlings was analyzed by measuring: fresh weight to assess the overall biomass of the plant, shoot length to indicate the growth of the aboveground portion, and root length to reflect the ability of the plant to anchor itself and absorb water and nutrients.
Statistical Analysis
Statistical analysis was carried out using SPSS software, adhering to the guidelines provided by IBM in 2009. The experiments were designed as completely randomized trials with three replicates, and they were analyzed as factorial experiments. To compare means, t-tests were conducted at a significance level of 5%.
Results
Primer Design and SbDHN1Gene Isolation
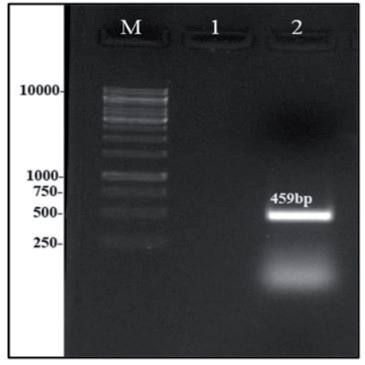
To amplify the SbDHN1 gene from Egyptian sorghum cultivar R12 plants, two specific primers were designed based on the mRNA sequence of S. bicolor dehydrin DHN1 (LOC8077913). The forward primer (F) sequence was 5’-GAATTCATGGAGTACGGTCAGCAGG-3’, and the reverse primer (R) sequence was 5’-GGATCCTTAGTGCTGTCCGGGCAG-3’. Utilizing these primers in an RT-PCR reaction, the full-length cDNA of the SbDHN1 gene (459 base pairs) was successfully extracted from R12 plants subjected to 200 mM NaCl stress (Fig. 1).
SbDHN1 Gene Characterization
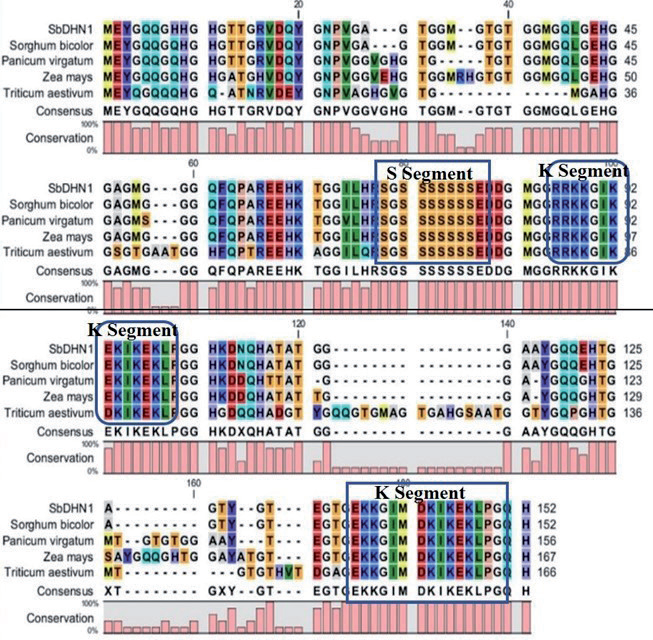
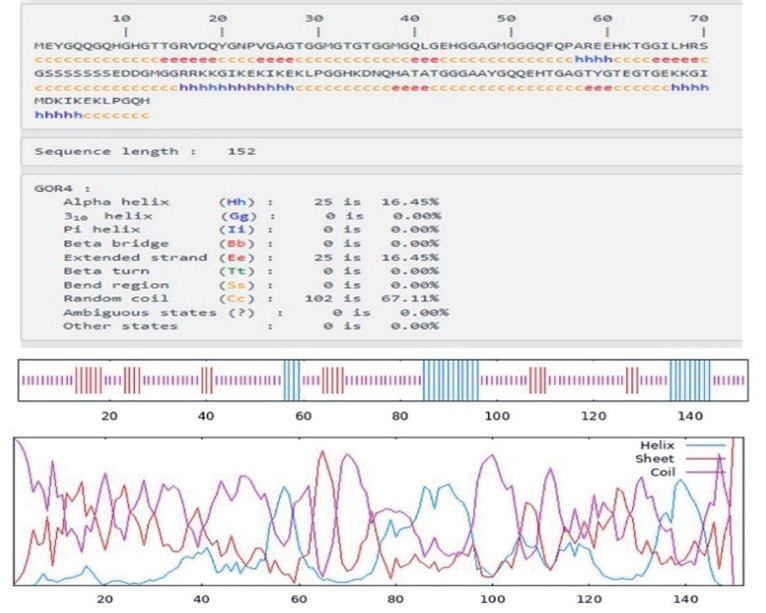
Following amplification, the SbDHN1 gene PCR product was sequenced and analyzed through a BLASTn search against available sequences in the NCBI database. This revealed high homology with DHN1 sequences from various species, including Sorghum bicolor (99.78%), Zea mays (86.65%), Panicum virgatum (85.74%), Hordeum vulgare (81.44%), Triticum aestivum (80.95%), and Oryza sativa (80.47%). The full-length cDNA of SbDHN1 (459 bp) was subsequently deposited in the GenBank database under accession no. OR462174.1. Further confirmation of successful gene isolation was achieved by translating the SbDHN1 nucleotide sequence into a putative amino acid sequence using the Expasy translator tool. This revealed a protein of 153 amino acids. Subsequent Blastp analysis of the deduced SbDHN1 protein sequence further supported sequence similarity with Sorghum bicolor (99.34%), Panicum virgatum (85.44%), Zea mays (85.02%), and Triticum aestivum (61.02%). The ExPASY online protein primary structure prediction server was utilized to analyze the primary structure of the SbDHN1 protein. This analysis revealed a length of 152 amino acids and a molecular weight of approximately 15.4 kDa (Fig. 2). In-depth analysis of the SbDHN1 protein sequence using bioinformatic tools revealed its molecular formula (C639H1017N211O222S6), amino acid composition (characterized by high Gly content at 27.6%, followed by Ala at 5.2%, Leu at 2.6%, and Arg at 3.3%), and isoelectric point (pI) of 8.81. This pI value indicates a net neutral charge for the protein at pH 8.81. Additionally, the estimated half-life of SbDHN1 was predicted to be lower than that of SbGly II, with values exceeding thirty hours in mammals, twenty hours in yeast, and ten hours in E. coli for SbGly II compared to a predicted instability index of 23.87 for SbDHN1. This suggests a potentially shorter lifespan for SbDHN1 protein, likely due to the slightly lower number of negatively charged residues (16 Asp+Glu) compared to positively charged residues (18 Arg+Lys). Analysis of the SbDHN1 protein’s hydropathy using the GRAVY score revealed a slightly hydrophilic character (-1.132). Prediction of its secondary structure with the GOR IV server indicated a composition of 16.45% alpha helices, 16.45% extended strands, and 67.11% random coils. Subsequently, multiple sequence alignment of SbDHN1 with other sequences using the CLC software identified the presence of conserved regions characteristic of SK2- type dehydrins. These conserved regions comprised two lysine-rich K-segments and one polyserine-rich S-segment, as visualized in Fig. 3.
Fig. 1.
The amplification of SbDHN1gene using RT-PCR. M: 1 Kb DNA ladder marker. Lane (1) represents the negative control and lane (2) represents the amplified gene.
Vector Construct
Following amplification, the SbDHN1 fragment was initially cloned into the pGEM-T vector for intermediate manipulation. Subsequently, the SbDHN1 gene was subcloned into the pCambia1390 expression vector utilizing the EcoRI and BamHI restriction sites. This resulted in the construction of the final pCambia1390-SbDHN1 vector depicted in Fig. 4.
Rice Transformation and Regeneration
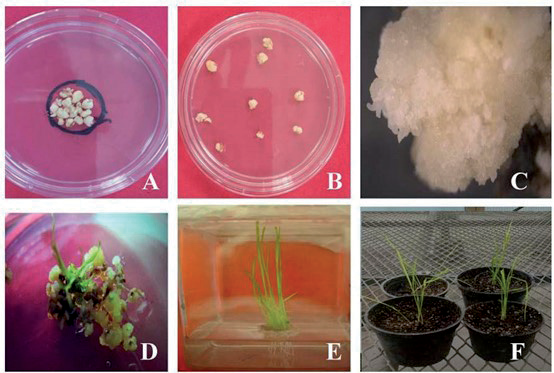
To generate transgenic rice plants expressing the SbDHN1 gene, biolistic particle delivery was employed. Two Egyptian cultivars, Giza 177 and Giza 178, were transformed using pCambia1390 containing SbDHN1 under the constitutive 35S promoter and Nos terminator. Transformation efficiency, calculated as the percentage of positive PCR-confirmed plantlets among bombarded embryos, was higher in Giza 177 (14.3%) compared to Giza 178 (12.3%) (Table 1). Harvested T0 plants yielded T1 seeds, which were sown in a bio-containment greenhouse to assess transgene inheritance (Fig. 5).
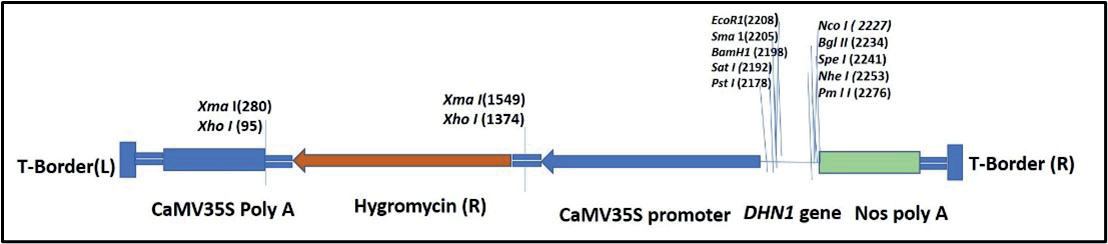
Table 1.
Transformation percentage of the two rice cultivars Giza 177 and Giza 178 using the SbDHN1 gene.
| Genotype | No. of bombarded Explants. | No. of survived calli | No. of plantlets | PCR confirmation | Mean % Transformation percentage |
|---|---|---|---|---|---|
| Giza 177 | 500 | 250a | 70a | 10a | 14.3b |
| Giza 178 | 500 | 300b | 65b | 8b | 12.3b |
Fig. 5.
Rice transformation, regeneration, and acclimatization stages. (A) calli after bombardment; (B) transformed calli after subculturing on selection medium containing 50 mg/l hygromycin (c) embryogenic calli; (D and E) shoot induction on regeneration medium; (F) acclimatization in the greenhouse.
Detection of Transgenic Rice
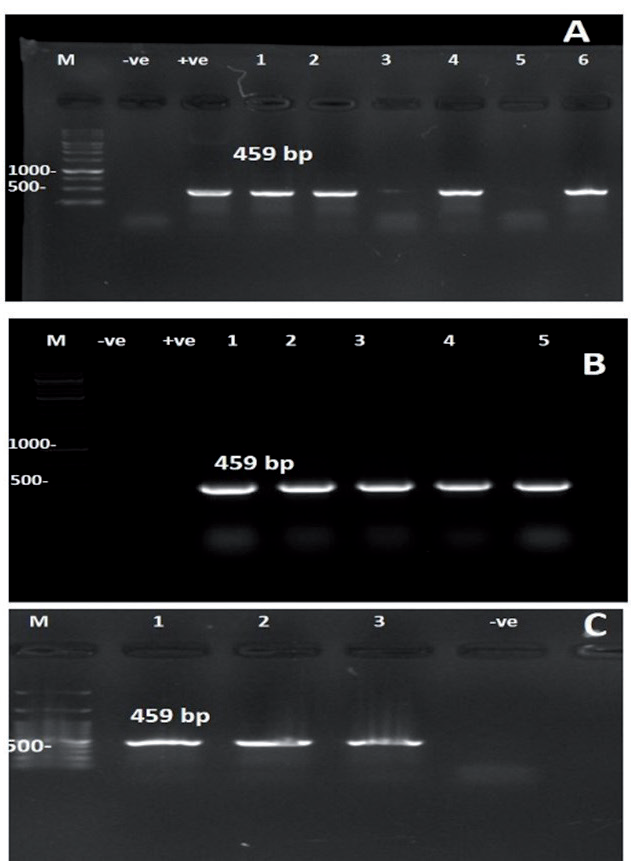
PCR amplification of the genomic DNA isolated from putative T0 rice transgenics with the SbDHN1 gene resulted in 459 bp products (Fig. 6A). No such amplification was found in untransformed control. Out of 135 individuals per line, 18 were found to be PCR positive. Among them, five T0 transgenics (M1, M4, M10, M15, and M16) were selected for further evaluation. T1 transgenics of these 5 lines were also found to be positive by PCR analysis using the SbDHN1 gene (Fig. 6B). PCR analysis of selected 3 T2 transgenic lines (M1, M4, and M10) using SbDHN1 gene-specific primers confirmed the carrying forward of the transgenes (Fig. 6C). Southern blot analysis in these transgenic lines further confirmed the stable integration of SbDHN1 (Fig. 7). Quantitative RT-PCR analysis of these 3 (M1, M4, and M10) transgenic lines using SbDHN1 gene-specific primers revealed that the transgenic line M4 had a high level of expression compared to M1 and M10 (Fig. 8).
Evaluation of T1 Rice Plants under Salt Stress Conditions
By subjecting transgenic T1 rice plants expressing the SbDHN1 gene to 200 mM NaCl, the plants’ ability to withstand salt stress was assessed. As summarized in Table 2 and visualized in Fig. 9, transgenic lines displayed a markedly higher growth rate compared to non-transgenic controls under salt stress. Significant variations in shoot length, root length, and fresh weight were found by statistical analysis comparing transgenic and non-transgenic plants expressing the SbDHN1 gene, suggesting that SbDHN1 may have a role in improving stress tolerance.
Discussion
Climate change predictions make it clear that immediate action is needed. Sustainable agricultural practices are urgently needed as the climate in this region is likely to have a negative impact on crop production. The development of stress-tolerant crops and the use of biotechnological innovations to improve the resilience of crops to rapid weather changes are essential for lasting food security. This work has shown that transgenic crops carrying stress-responsive genes such as SbDHN1 could alleviate salt stress in rice. The mechanism of stress resistance is significantly enhanced. We want to understand dehydrin gene families such as SbDHN1 and elucidate the molecular mechanisms of plant response to abiotic stress.
Dehydrins, a type of LEA (Late Embryogenesis Abundant) protein, play an important role in the plant’s response to drought, cold, salinity, and heat. The original identification of barley and maize DN cDNAs was based on their response to dehydration, ABA, or salt stress. This identification has greatly improved our understanding of the molecular functions of DHN genes. The existence of DHN genes in many plant species gives them great importance from an evolutionary point of view. Functionally defined DHNs have shown improved resistance to abiotic stress in crop plants, including rice. Their presence has also been found to have positive effects in model plants such as Arabidopsis, as well as in wild species living in extreme environments. The way in which DHNs become adaptive in halophytes, resurrection plants, drought-tolerant species, and hardy plants suggests their potential to maintain plant resilience under various challenging stimuli. Understanding DHN genes and their functions offers advanced biotechnological solutions to improve crop resilience and food security around the world in the face of climate change.
Fig. 6.
Transformation confirmation of transformed rice plants. A: PCR confirmation for T0 rice plants. B: PCR confirmation for T1 rice plants. C: PCR confirmation of the SbDHN1 gene of T2 transgenic rice. M: 1 Kb DNA ladder marker. Lanes (1, 2, 3, 4, 5, and 6) represent putatively transformed rice plants; Lane (-ve) (non-transformed rice) negative control; Lane (+ve) (pCambia1390- SbDHN1 vector) positive control.
The successful isolation and cloning of the SbDHN1 cDNA sequence from sorghum into the plant expression vector pCambia1390 have provided the first look at the structural and functional properties of dehydrins, in particular this species -SbDHN protein. The SbDHN protein sequence is rich in specific amino acids typical of dehydrins, such as alanines and glycines; leucines and arginines are particularly prominent according to this model document [28]. With its DLC- and polyserine-rich S segment, the solubilized SbDHN fits into the classification of SK2-type dehydrins [29]. The introduction of the SbDHN1 gene into the rice varieties Giza 177 and Giza 178 and the subsequent tests under 200 mM NaCl stress in vitro showed a significantly improved growth of the transgenic lines compared to the non-transformed controls. These results confirm the hypothesis that overexpression of DHN increases resistance to several abiotic pathogens [19]. Studies have shown that dehydrins such as SbDHN1 help plants to survive hot temperatures and drought stress [30]. In addition, transgenic studies on the overexpression of dehydrins have shown that tolerance to low temperatures, drought, and osmosis is increased. The protective effect of dehydrins against oxidative stress has also been confirmed in transgenic tobacco plants [31]. However, more recent studies have repeatedly shown that dehydrins can protect plants from harsh environmental conditions. For example, transgenic rice transformed with OsRab16A dehydrin showed increased tolerance to salt [28]. RcDHN5 from Rhododendron and DHN24 from Solanum in transgenic Arabidopsis and cucumber seedlings resulted in a significant improvement in cold and frost resistance [32]. The leaves of many genetically modified tobacco, rice, and Arabidopsis plants show signs such as salt tolerance. High osmotic and drought conditions enhance this tendency in plants already equipped with endogenous dehydrins as a biomolecular mechanism for defense against abiotic stress [19]. Tobacco plants transformed with Brassica juncea BjDHN2 or BjDHN3 dehydrins were found to be tolerant to heavy metal stress, especially Cd2+ and Zn2+. When exposed to low temperatures, drought, or high salinity, dehydrins accumulate as LEA proteins [33, 34]. These proteins are essential for maintaining cell homeostasis and help plants in the field. Under stress conditions, dehydrins accumulate and are also involved in the regulation of proline metabolism and reactive oxygen species (ROS) scavenging systems, giving plants greater stress resistance [19].
Fig. 7.
Southern blot analysis Lane 1-5 transgenic lines M1, M4, M10, M15, and M16, respectively, and lane (-ve) untransformed control.
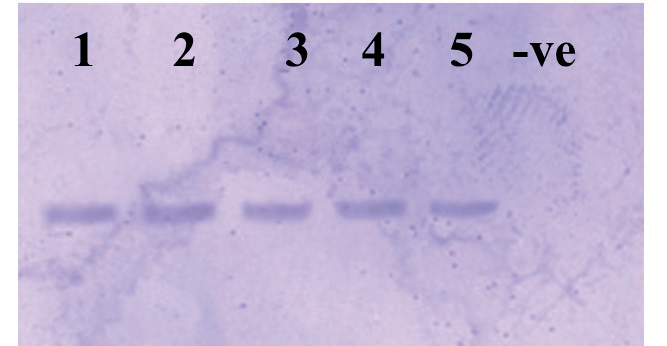
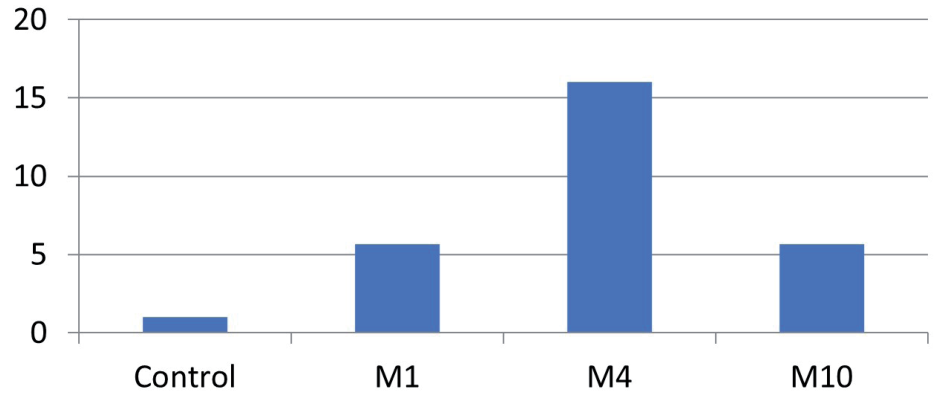
Fig. 9.
The shoot and root growth of transgenic rice cultivars compared to the non-transformed plants. (A): Cultivar Giza 177 and (B): Cultivar Giza 178. The (T) for transformed plants and (C) for control (non-transformed plants).
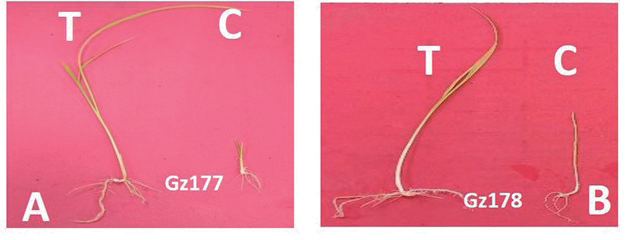
Table 2.
Shoot length, the root length, and the fresh weight for transformed rice cultivars compared to the non-transformed plants.
Conclusions
The SbDHN1 gene plays an important role in increasing the salt stress resistance of the transgenic rice lines Giza 177 and Giza 178. By successfully isolating, cloning, and transferring the SK2-type dehydrin gene from Egyptian sorghum into rice, this project has not only highlighted biotechnology in agriculture but also the potential of genetics to improve crop resistance. This study has many strengths; these include a detailed characterization of the SbDHN1 gene, a well-established transformation process, and a comprehensive evaluation of the transgenic rice under salt-pressure-free conditions. In contrast, there is clear evidence of the salt tolerance conferred by the SbDHN1 gene through the growth parameters observed in the transgenic lines compared to the control plants, including shoot length, root length, and fresh weight, all of which were greater in the transgenic line. These results provide further insights into the functions of dehydrin; they are therefore also helpful for the improvement of plants. By mastering the material and energy forms of dehydrins, researchers can develop creative strategies to increase the stress tolerance of crops. Such strategies support sustainable farming practices and help address global food security issues caused by climate change. In the coming times, genetic engineering or biotechnology will continue to advance and will certainly be the decisive factor that determines the future of agriculture.

