

Introduction
Antibiotics, known for their therapeutic efficacy, have found extensive application in human medicine, aquaculture, and livestock farming [1]. They are often directly expelled from these living organisms into the broader environment [2, 3]. The accumulation of residual antibiotics in the natural environment may exert selection pressure on microorganisms [4], leading to increased propagation and dissemination of antibiotic resistance genes (ARGs), although they occur naturally [5, 6]. Over the past several decades, ARGs have been identified as a novel but ever-growing category of environmental pollutants on a global scale [7, 8]. Every year, antibiotic-resistant bacteria contribute to approximately 700,000 fatalities, posing a significant health threat and economic challenge, particularly in economically developing regions [9].
ARGs have been detected in a wide range of environmental matrices, particularly aquatic ecosystems that are more susceptible to anthropogenic activities [10, 11]. Serving as pivotal contributors to ecosystem services, lakes are significant terrestrial repositories for both antibiotic-resistant bacteria and ARGs [12]. Domestic and livestock wastewater channels antibiotics into the lakes, thus amplifying the levels of antibiotics and ARGs [13, 14]. Concurrently, ARGs are able to remain in the lakes with long retention intervals [15], and create more opportunities for the emergence of resistant pathogens [13]. Consequently, it is both urgent and critical to comprehend the occurrence and transmission of ARGs to thwart and manage their pollution risk in the lakes.
Five tributaries, namely the Gan, Fu, Xin, Rao, and Xiushui rivers, flow into Poyang Lake [16], forming the largest freshwater system in China and the most important aquatic resource serving the local ecosystem and economy [17]. In recent times, the emergence of various contaminants, including antibiotics and ARGs, has seriously affected the ecological environment of Poyang Lake [18]. Yet, there are still gaps in understanding the environmental risks of ARGs and associated microorganisms in Poyang Lake, and the contribution of different tributaries to the occurrence of ARGs. To date, only one literature has reported on the characterization of ARGs in the surface water of Poyang Lake using gene amplification-based techniques (e.g., quantitative PCR) [19]. Although the data obtained from this study was relatively limited, it still indicated the possible pollution risk of ARGs. Compared with methods based on gene amplification, metagenomic analysis can offer comprehensive and in-depth insights into the distribution and composition of ARGs and related microorganisms in natural environmental samples [11, 20]. To our knowledge, metagenomic techniques have been used to investigate microbial communities and ARGs distribution in a variety of aquatic ecosystems, including Kazipally Lake [21], Tai Lake [15] and Qinghai Lake [13], with great success.
Fig. 1.
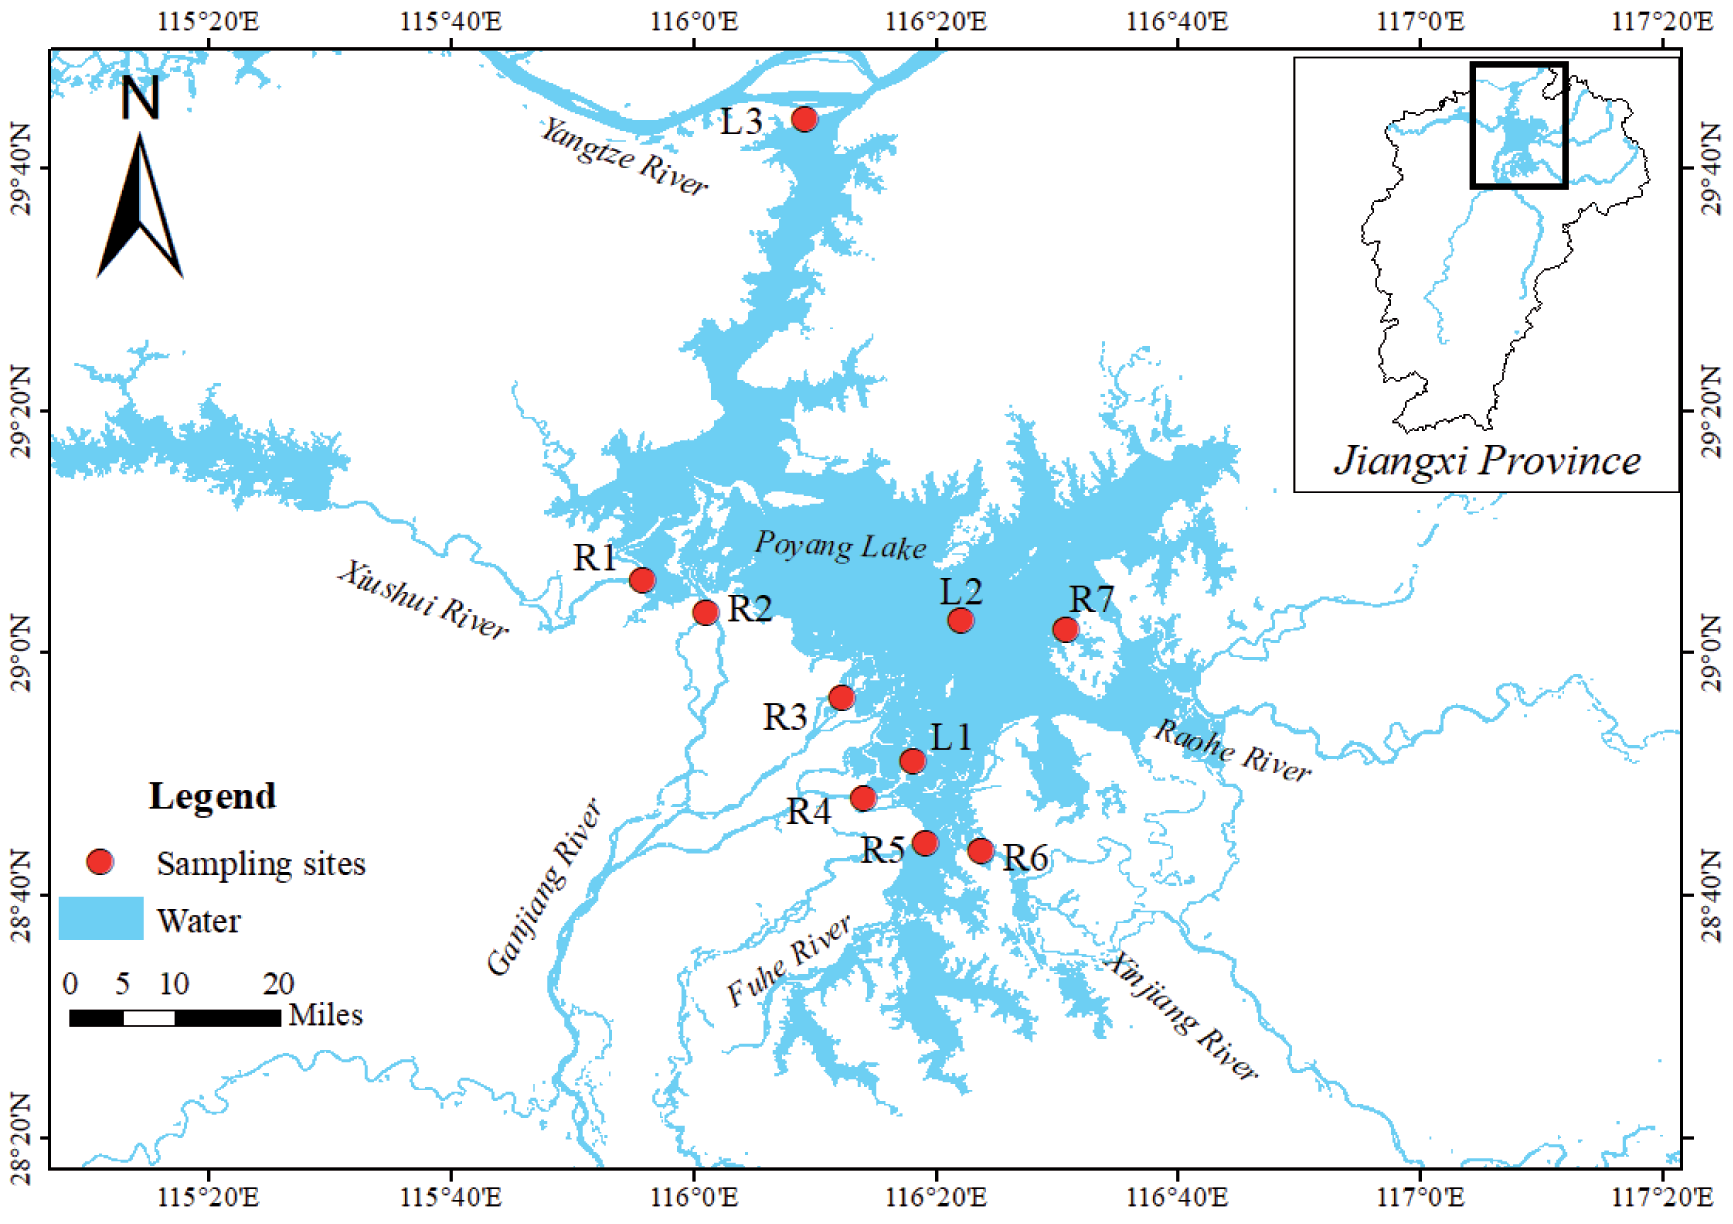
A map of sampling sites. R1, the Xiushui River; R2, the north branch of the Gan River; R3, the middle branch of the Gan River; R4, the south branch of the Gan River; R5, the Fu River; R6, the Xin River; R7, the Rao River; L1, the Nanjishan Wetland National Nature Reserve; L2, center of Poyang Lake; L3, the outlet sites of Poyang Lake into the Yangtze River
Therefore, the objective of the present study is to comprehensively understand the current situation of ARG pollution in Poyang Lake by using metagenomic analysis as the primary investigative tool. Accordingly, the structure and dispersion of ARGs, and microbial communities in both the surface water and the sediment, were investigated. The results are expected to provide a reasonable assessment of ARG pollution risk in Poyang Lake, thereby contributing to the formulation of mitigation strategies to curb their widespread propagation.
Material and Methods
Sample Collection
According to our previous work [17], we gathered samples from both the surface water and sediments of Poyang Lake in November 2021, across a five-day span devoid of rainfall. Ten locations, representing the lake’s entire geographical expanse, were selected for sampling (Fig. 1). Notably, seven sites (R1~R7) were situated in the five tributaries feeding into Poyang Lake. Sites L1 and L2 were dispersed within the Nanjishan National Nature Reserve and the central region of Poyang Lake, respectively, while site L3 was positioned at the junction where Poyang Lake drains into the Yangtze River.
At each site, three 1L replicates of surface water were collected using pre-sanitized stainless-steel buckets and subsequently stored in sterilized plastic bottles. In parallel, three replicate samples of surface sediments, each weighing approximately 1 kg and extracted from a depth of 10 cm using stainless steel Petersen samplers, were sealed in sterile polypropylene plastic bags. All samples were instantly refrigerated, transported to the laboratory on dry ice within a 24-hour window, and preserved at -80 °C pending analysis.
DNA Extraction and Shotgun Sequencing
The antibiotic sample analysis was performed using ultra-high-performance liquid chromatography-tandem triple quadrupole mass spectrometry (UPLC-MS/MS, US, Agilent) based on the previous research [22].
Surface water samples were vacuum-filtered through a 0.22 μM filter membrane (SCBB-206, ANPEL, China), with the resulting membrane promptly transferred to a sterilized centrifuge tube for instantaneous flash-freezing in liquid nitrogen. Subsequently, DNA was extracted from the material on the filter membrane utilizing an E.Z.N.A.™ Water DNA Kit (OMEGA Bio-Tek, USA). Concurrently, genomic DNA was harvested from each sediment sample (0.25 g) using a Soil DNA Kit (OMEGA Bio-Tek, USA), in accordance with the manufacturer’s instructions. DNA quality was assessed through gel electrophoresis, and all extracted samples were preserved at -20 °C until further use. The harvested DNA samples were then ultrasonically fragmented into 250–300 base pair segments. These DNA fragments underwent end-polishing, A-tailing, and ligation with dual-index adaptors in preparation for Illumina sequencing, followed by additional PCR amplification.
Metagenome Assembly and Species Annotation
High-throughput sequencing was conducted on the Illumina Hiseq 2000 platform, employing a paired-end (2×150) sequencing approach. FastQC software was used to assess the base quality of the original sequencing data [23]. Megahit assembled the high-quality reads sequences metagenomic, with the minimum sequence length ≥500bp for each sample [24]. High quality filtered reads were compared to MetaPhlAn2 database to obtain sample microbial species composition and abundance information. Reads not assembled in each sample were combined and assembled again [25]. The assembly mode is “meta-sensitive” and the assembly sequence is preserved at least 100bp. Prodigal was used to predict metagenomic protein-coding genes, and CD-HIT was used to construct non-redundant gene sets [26].
Antibiotic Resistance Gene Annotation
Given the diversity of bacterial, archaeal, viral, and eukaryotic genomes, MetaPhlAn2 has been recognized as a valuable tool for elucidating microbial community structure in metagenomic data [25], owing to its ability to distinguish hosts based on 1M unique marker genes found within those reference genomes. Clean reads were matched against precompiled marker catalogs derived from existing microbial genomes using the nucleotide aligner Bowtie2, enabling us to obtain taxonomic information about our samples.
To predict resistomes, the sequence of the metagenomic gene catalog was subsequently aligned with the Comprehensive Antibiotic Resistance Database [27], given the extensive array of known ARGs and their corresponding resistant drugs housed in the database. To ensure the precision of ARG identification, a cutoff of 80 percent was selected as the search parameter [28].
Statistical Analysis
Statistical analyses were carried out employing R (v3.5.2), utilizing packages such as vegan, car, and GUniFrac. One-way ANOVA was conducted to determine the significance of differences in ARG abundance across various sites, with a p-value of less than 0.05 deemed statistically significant. Principal Coordinates Analysis (PCoA) was utilized to discern correlations or distinctions between variables and/ or samples. To probe the overall correlations between ARGs [28] and the microbial community, Procrustes analysis was implemented. Metagenomic data are provided in the National Microbiology Data Center (Accession number: SUB1686727741190).
Results and Discussion
Occurrence of Antibiotics
The accumulated concentration and detection frequency of the 13 antibiotics at 10 sampling sites in Poyang Lake are compiled in Table 1. The majority of target antibiotics were identified in the water samples, indicating a widespread presence in this region. Tetracycline (TC), oxytetracycline (OTC), chlortetracycline (CTC) and sulfadiazine (SDZ) were the most commonly identified antibiotics, with detection frequency of 95%, 85%, 85%, and 75% in the surface water samples, and of 80%, 75%, 65%, and 60% in sediment samples, respectively. The total concentration of the detected antibiotics ranged from 13.8 ng L-1 to 237.7 ng L-1 (mean 78.5 ng L-1) in surface water samples, and from <8 ng g-1 to 73.2 ng g-1 (mean 32.2 ng g-1) in sediment samples. As reported, the antibiotic concentration reached 917 ng/L in groundwater in urban areas [29] and 19.68- 497.00 ng L-1 in a drinking water source in East China [30]. In the sediment, the concentration of the antibiotics was from 23.73 to 126.46 ng g-1 in Awash River Basin, Ethiopia [31]. Taken together, the Poyang Lake ecosystem was polluted by a variety of common antibiotics, but the degree of pollution was relatively light.
Microbial Community Structure
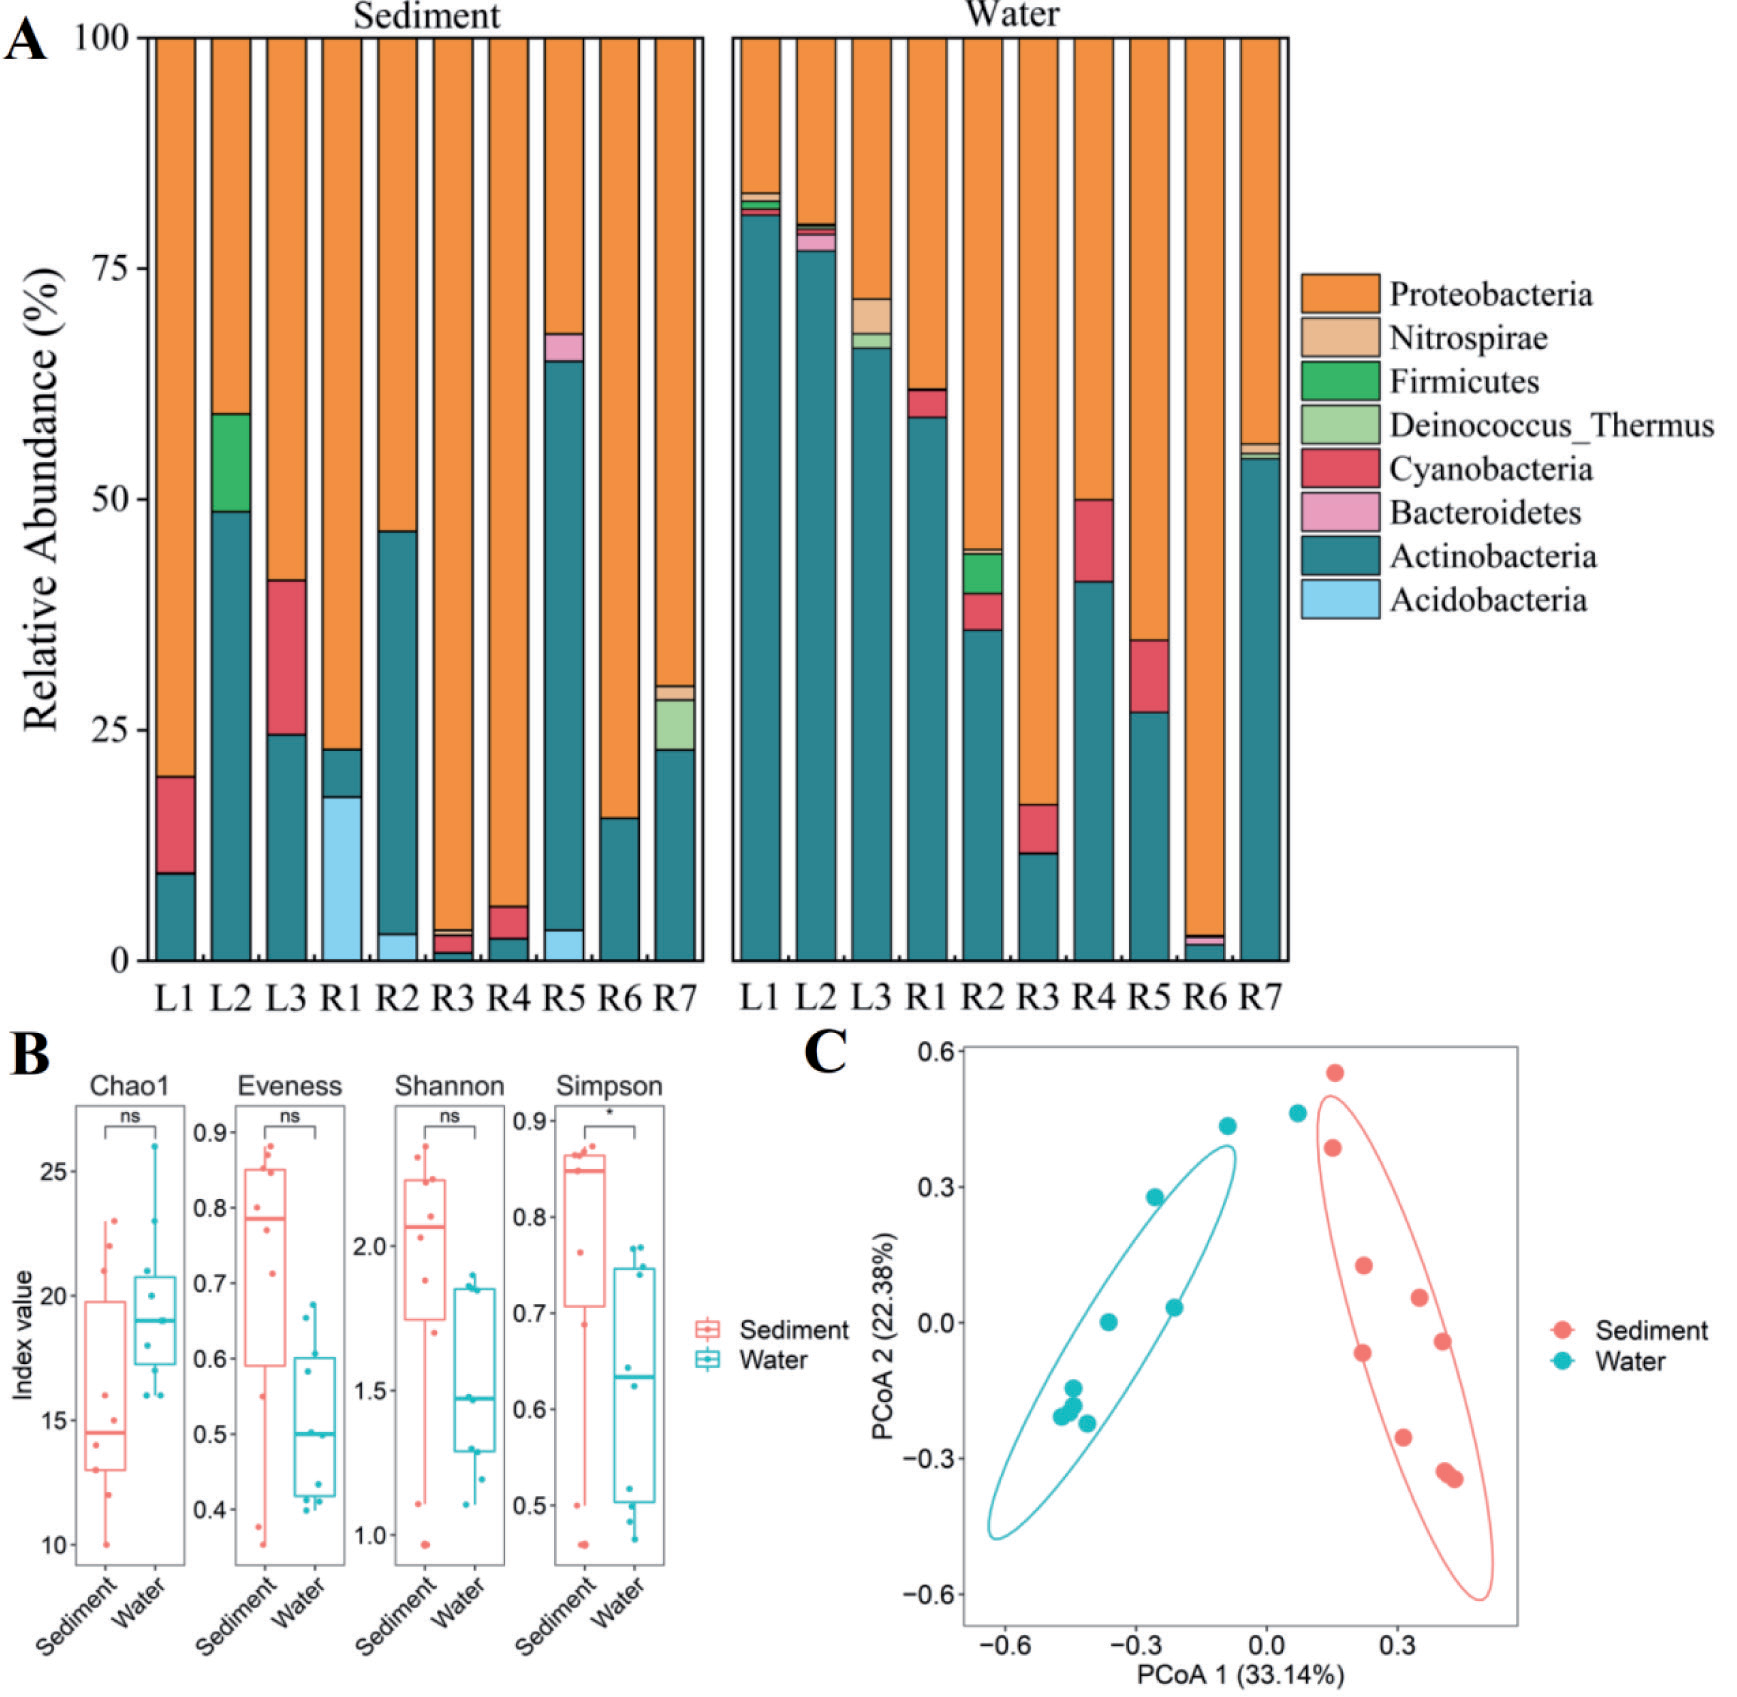
Data acquired from all test specimens were categorized into eight distinct branches at the phylum, revealing a unique bacterial blueprint for each instance. The phylum Proteobacteria demonstrated the greatest abundance in sediment samples from sites R1-R7 and L3, accounting for 50.2% to 97.3% of the total, while Actinobacteria was the most enriched phylum in sediment samples from sites L1 (61.65%) and L2 (48.66%). For surface water samples, Proteobacteria and Actinobacteria emerged as the dominant phyla, representing 82-100% of the complete bacterial society (Fig. 2A). This finding was similar to previous reports. For instance, Proteobacteria, Bacteroidetes, and Actinobacteria made up over 80% of the total microbial community in water from a mariculture system [32]. Proteobacteria, Chloroflexi, and Acidobacteria were the most abundant under phyla level in the estuaries [10]. Proteobacteria were also the most dominant bacterial phylum in wastewater treatment plants (WWTPs), Tai Lake and Qinghai Lake [13, 15, 33]. It suggested that Proteobacteria and Actinobacteria appeared to be the main microbial colonizers of natural substrates in aquatic environments [34].
Examining the diversity indices (α-diversity and β-diversity) of microbial societies between surface water and sediment selections offered additional insight. The α-diversity indices, which include observed Chao1, Evenness, Shannon, and the Simpson index, indicated a significantly greater diversity of microorganisms in sediment instances compared to corresponding water samples (Fig. 2B). Moreover, a Principal Coordinates Analysis (PCoA) grounded on the Bray-Curtis distance unveiled the disparity in bacterial societies between sediment and water samples (R2 = 0.28, P < 0.001, Fig. 2C). This was consistent with our common understanding that the sediment is a major reservoir of microorganisms [35].
ARGs Composition
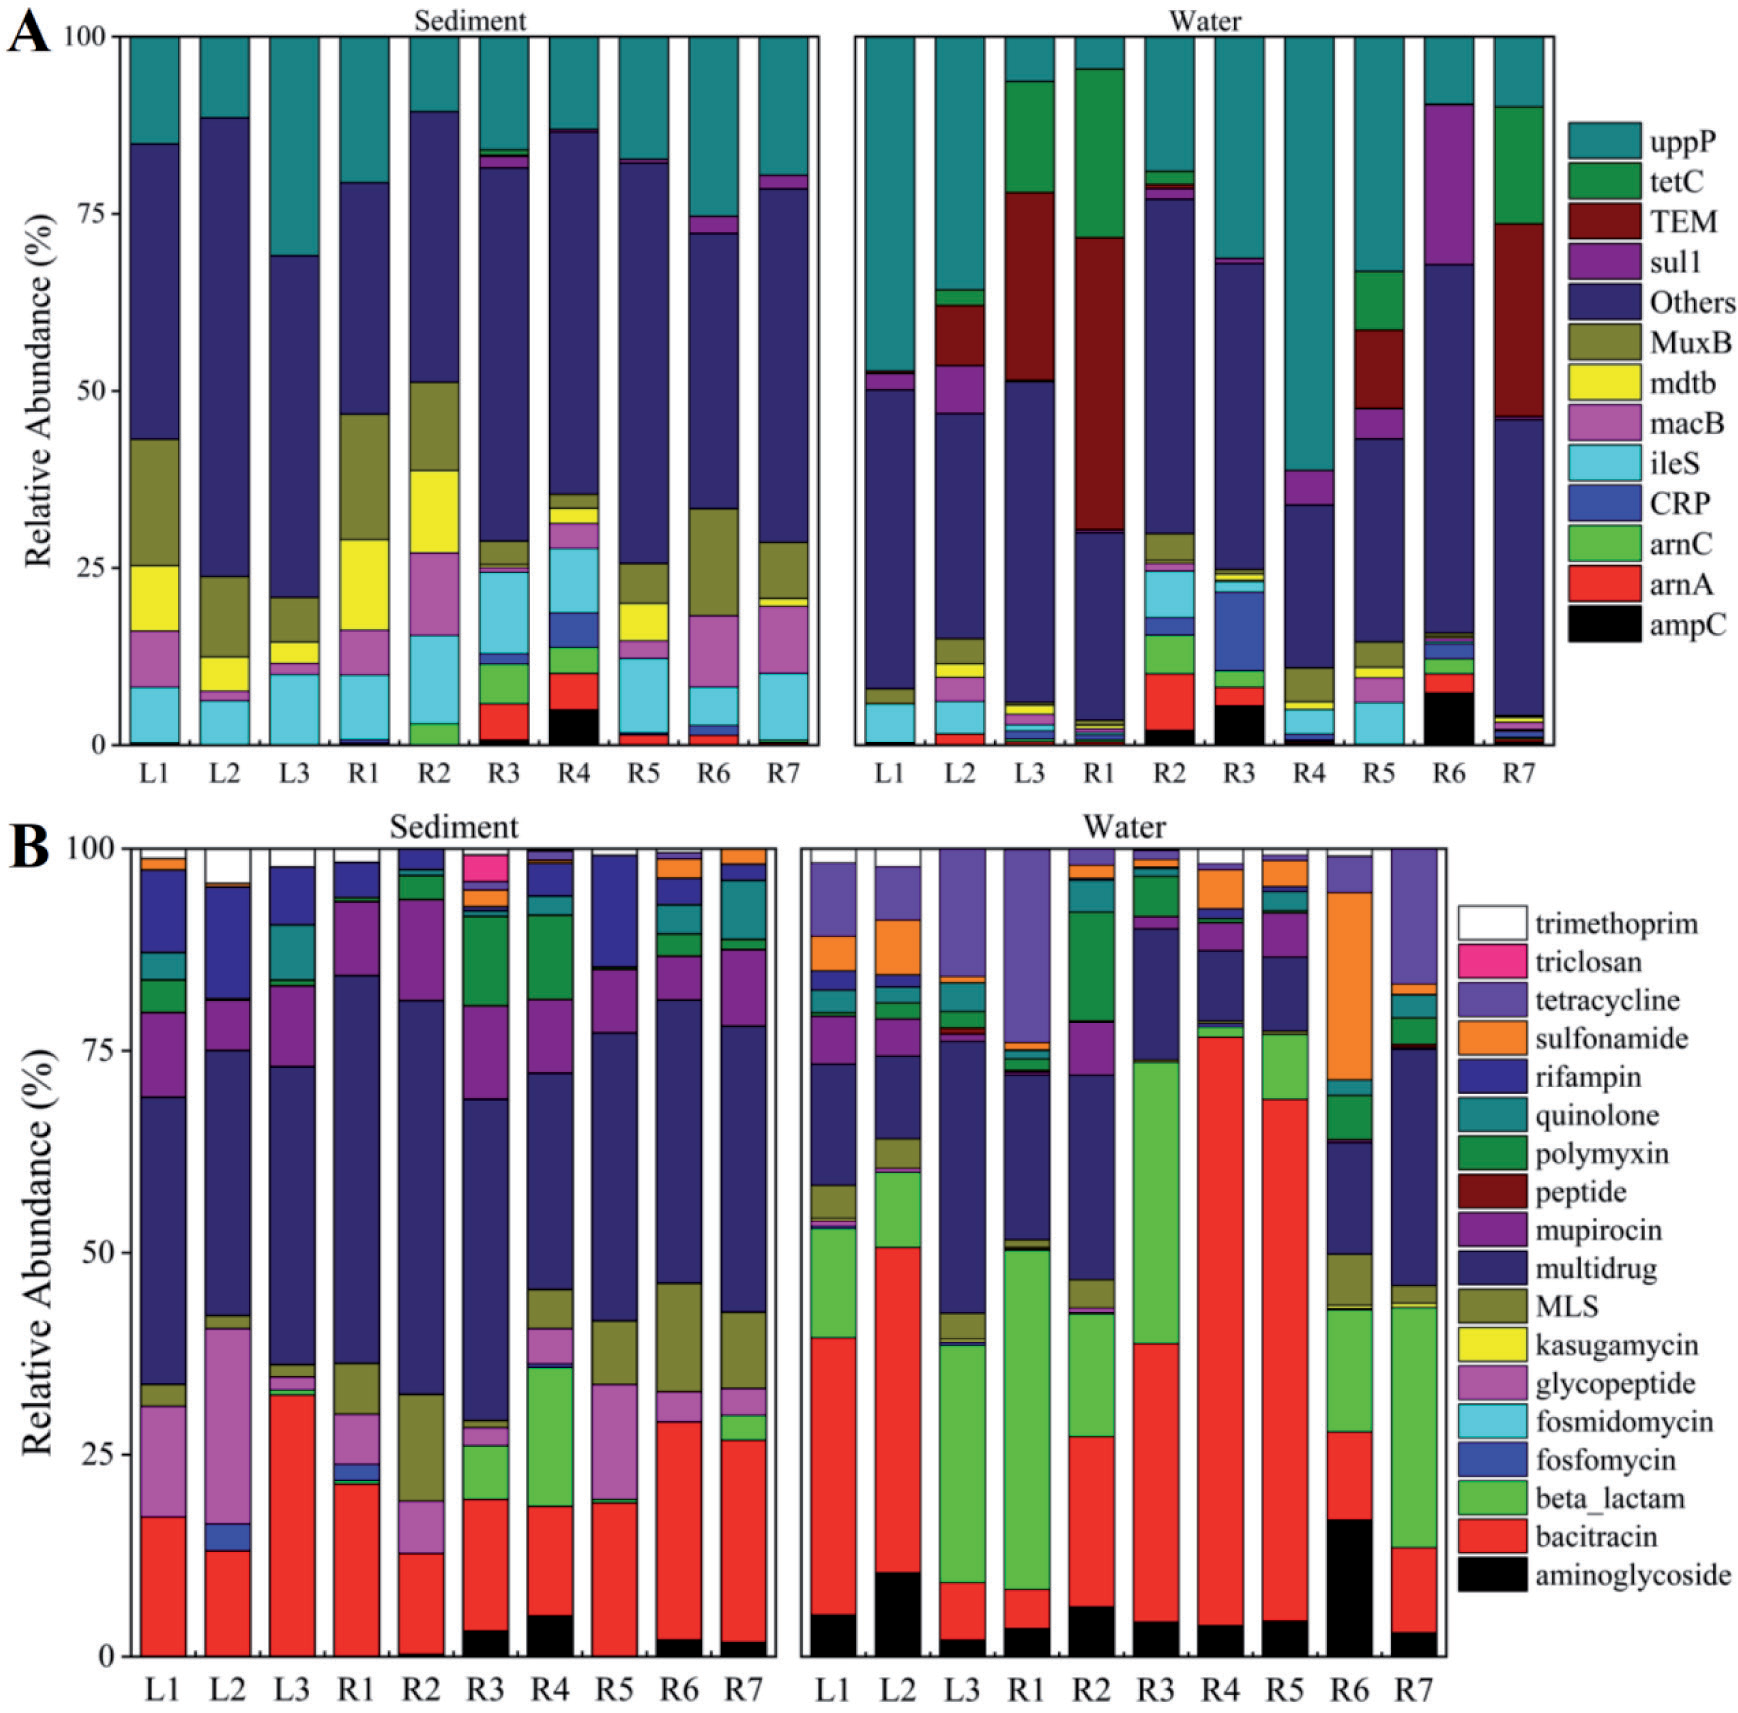
Eighteen forms of ARGs were extensively identified in the surface water and sediment specimens from Poyang Lake, with 15 specific types for surface water and 17 for sediments. Bacitracin, multidrug, and mupirocin were the top three most abundant ARG types in the sediment samples, while multidrug, β-lactam, bacitracin, and tetracycline were the most prevalent genes in the surface water samples. Among them, the most dominant ARG type was multidrug for all water and sediment samples (Fig. 3B). In previous studies, multidrug was most frequent in urban environments [20], the drinking water supply system [36], estuaries [37], urban-lake drinking water [38], as well as WWTPs [33]. The highest content in the sediment of Tai Lake was the multidrug, followed by macrolide-lincosamide-streptogramin (MLS), and bacitracin [15]. These results aligned with our study, which was unsurprising given the ubiquity of multidrug resistance efflux pumps in prokaryotes [39]. Nevertheless, a prior study by Liang et al. (2020) indicated that sulfonamides were the dominant antibiotics in the surface water of Poyang Lake [19]. Ding’s study identified that aminoglycoside and multidrug were the most frequent resistance genes in sewage treatment plants adjacent to Poyang Lake [22]. The conflicts between the results may exist due to the different analysis methods and sampling time.
Table 1.
The concentrations and detection frequencies of the 13 antibiotics in water and sediment in Poyang Lake
Fig. 2.
Histogram of species distribution of bacteria (a) in water and sediment at the phylum level (A); the diversity indices of microbial communities between sediments and water (B); Principal Coordination Analysis (PCoA) of bacterial communities between sediments and water (C)
The top 12 dominant ARG subtypes, including uppP, tetC, TEM, sul1, MuxB, ileS, ampC, arnA, macB, CRP, mdtb, and arnC, accounted for the abundance ranging from 23% to 74%. Moreover, uppP, tetC, and TEM-33 were the top three most abundant subtypes in the surface water samples, while uppP, MuxB, and ileS in the sediment samples (Fig. 3A). Among the ARG subtypes, the uppP, MuxB, and ileS posed high risks to human health [40]. In comparison, sul2 and qnrD were identified as the predominant resistance genes in Kazipally Lake, India [21]. Genes macB, uppP, ileS1, and mfd were the preponderant ARGs in sediment samples from Tai Lake, while bacA was the primary one in water of Chao Lake [38]. The gene sul1 was found to be dominant in the sediments of the sea area adjacent to the Yangtze Estuary [9]. In our study, uppP was the most abundant ARG, contradicting a recent report that failed to detect uppP in the surface water of Poyang Lake using qPCR [19]. The discrepancies might arise from inconsistent results of resistance genes between qPCR quantitative, and metagenomic sequencing data. qPCR can only detect preset target genes, which makes it easy to miss some important genes. The uppP gene was not determined in Liang’s study. Thus, the selected resistance genes for qPCR quantification may not comprehensively capture the level of bacterial antibiotic resistance within each sample [41].
Distribution of ARGs
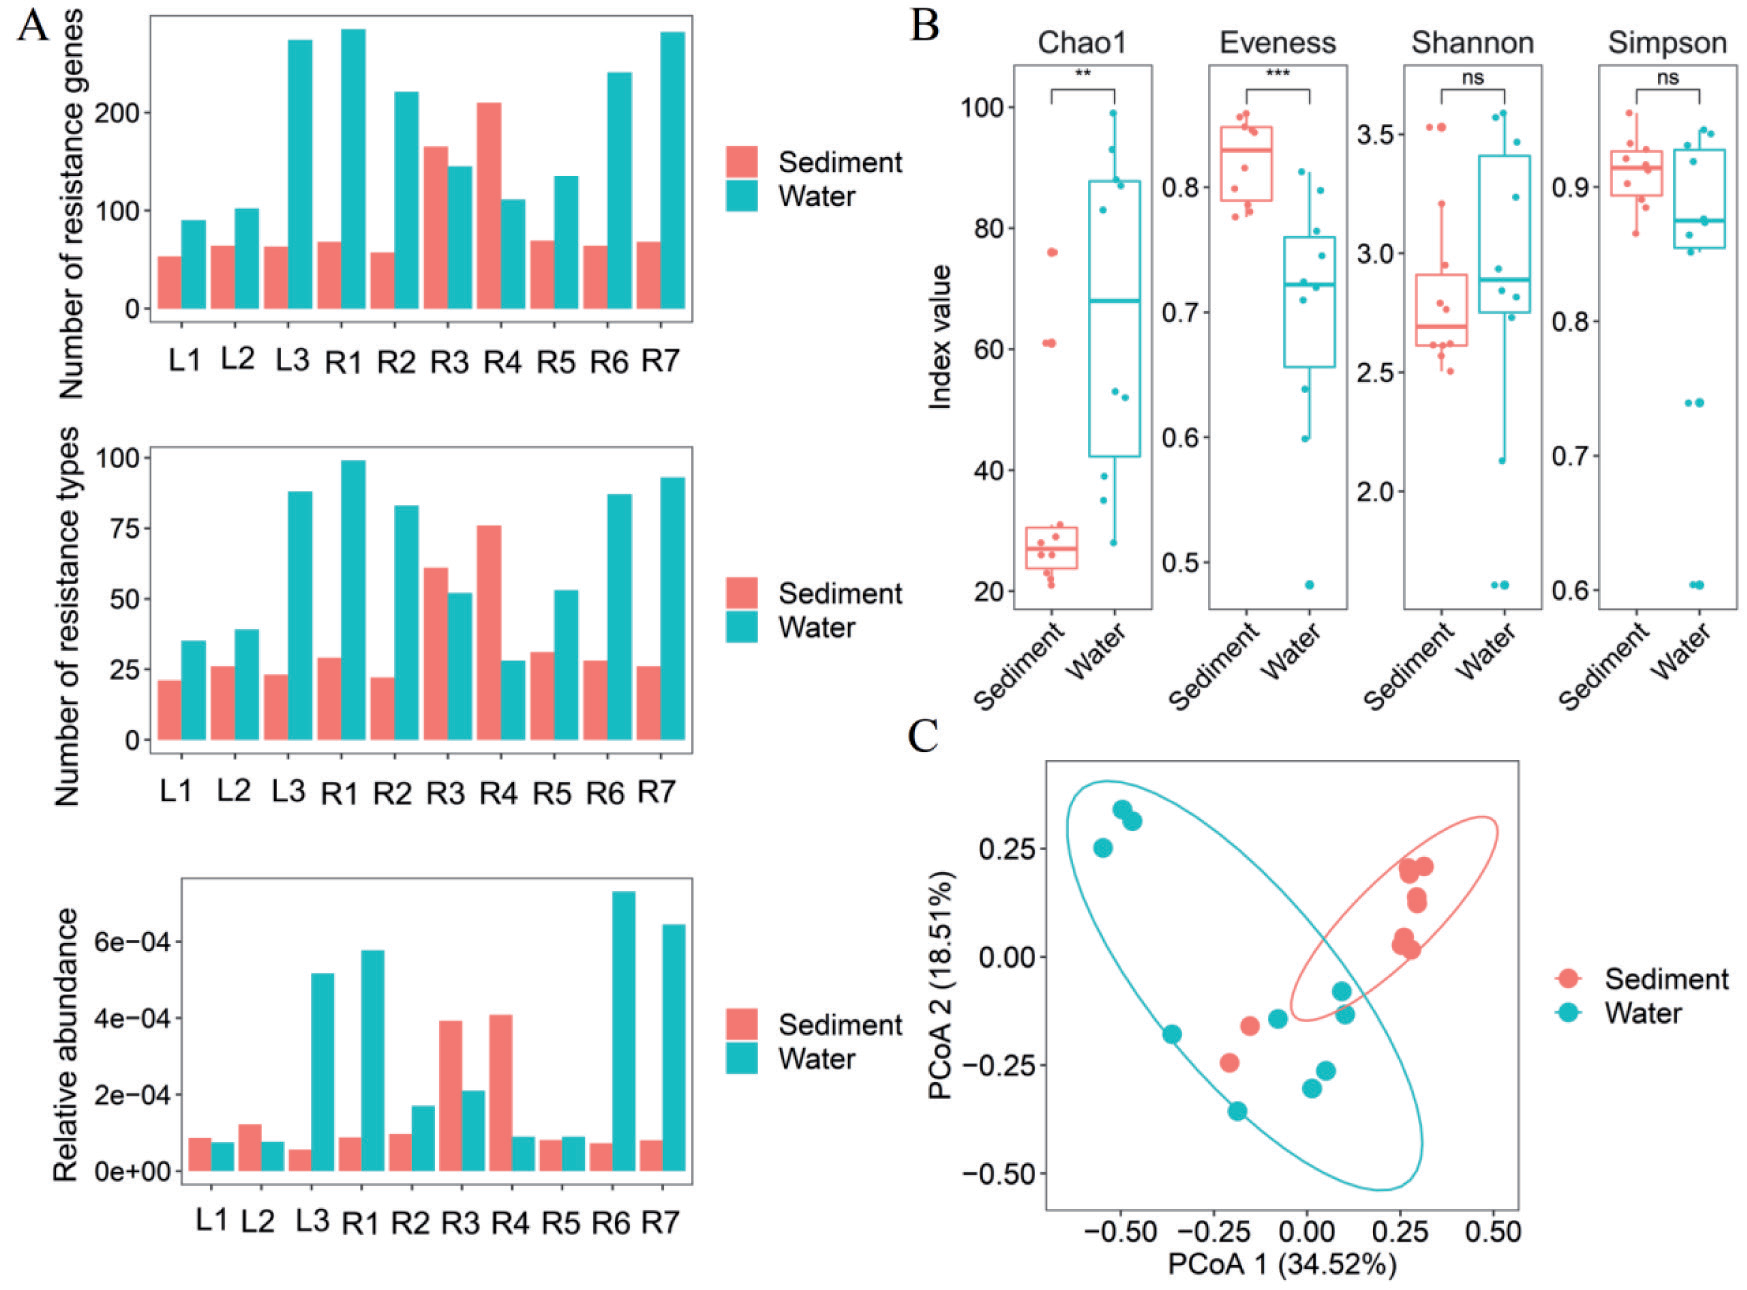
In the examination of surface water and sediment samples, there was a noticeable divergence in the count of ARG subtypes. The water samples from sites R1, R2, R5, R6, R7, L1, L2, and L3 hosted a greater variety of ARG subtypes compared to their sediment counterparts, as illustrated in Figure 4A. A contrasting trend was observed at sites R3 and R4. An analysis of ARG abundance across different sites indicated that the sediments from sites R1, R6, R7, and H3 contained the highest ARG abundance. A variety of indices for α-diversity related to ARGs were assessed in both surface water and sediment samples. The Chao1 index demonstrated a markedly higher value in surface water than the sediment (Fig. 4B). Each category of ARGs was linked with its corresponding antimicrobial agent, enabling a summary of the relative profusion of categories resistant to the identical antimicrobial agent. The Principal Component Analysis (PCA) of ARG profiles was executed to scrutinize the spatial variances in surface water and sediment specimens. As illustrated in Fig. 4C, the initial two components of PCA accounted for 52.26% of the variation in overall ARG abundance, and a clear distinction was observed between surface water and sediment samples in the PCA axes. This indicated that matrix played a substantial role in the dissimilarity of ARG composition.
ARGs in the sediment showed a decreasing trend from inlet to outlet of Poyang Lake, while an opposite result was found in sediments from the Yangtze Estuary [42]. While in the water, the relative abundance of ARGs increased first, and then decreased from inlet to outlet. Previous studies indicated a descending order of sul2 and tetA absolute concentrations at various sampling sites: tributary rivers > Yangtze River > Poyang Lake [19]. The variations in ARG profiles between the spatial gradient across the lake, from inlet to the outlet, might be influenced by the inflowing rivers. Our study revealed that the ARGs in sediment of the middle branch of the Ganjiang (R3) and the southern branch of the Gan River (R4) were higher than other regions. This may be because the Gan River flows through the entire district of Nanchang, one of the most densely populated areas in Jiangxi Province with large amounts of antibiotics used in human medicine, animal farming, and agriculture in this region. The spatial variation of ARGs in Poyang lake was interpreted as the more susceptible to human activities of the inlet of the Lake. We found less abundant ARGs in Nanjishan (L1), probably due to Nanjishan’s well-known national nature reserves, which are less disturbed by human activity. This suggested the role of anthropogenic activities in the ARG prevalence in this region [43]. ARG levels in aquatic ecosystems are thought to be closely related to human activity [44, 45]. The high consumption of antibiotics in densely populated areas is a result of their extensive use in human therapy, veterinary medicine, and as growth promoters in livestock farming, which has been shown to exacerbate ARG levels. Human-induced waste, including household sewage and hospital wastewater, significantly contribute to the dispersion of ARGs in the Lake [46-48].
Factors Affecting ARGs
The distribution and prevalence of ARGs are contingent upon a confluence of factors. Among them, microbial community and MobileGenetic Element (MGEs) have been considered as the two major direct factors [38], because microorganisms are the predominant source of ARGs [49] and exhibit potential for promoting the horizontal transfer of ARGs via MGEs [50, 51].
Procrustes analyses were performed to evaluate the effect of bacterial community on the composition of ARGs existing in Poyang Lake. The result showed that bacterial community composition has shaped the resistome (P < 0.01, Pearson’s correlation 0.7, Fig. 5), indicating that the composition of ARGs was highly dependent on the microbial community. This was in agreement with previous reports. Microbial community was reported to be the most important factor determining the antibiotic resistome along a drinking water supply system [36]. Bacterial communities could influence the composition of ARG hosts [52, 53]. Specific bacterial phyla, namely Proteobacteria and Acidobacteria, were the primary ARG hosts [11, 30]. Proteobacteria, the dominant phylum in the sediment across numerous sites in Poyang Lake, has been demonstrated to host most of the investigated plasmids and chromosomal integrons [54]. Actinobacteria were reported to possess the genetic capability to produce a wide range of antibiotics and accommodate diverse ARGs [55], as they are closely related to the ARGs [56]. Thus, these findings underscore the impact of bacterial communities on the composition and dispersion of ARG hosts, which in turn shape the characteristics of ARGs.
To corroborate the possible mobility of ARGs, a multitude of ARGs residing within the assumed mobile elements in the same metagenomic contigs were discovered (Fig. 6A). A broad spectrum of MGEs series was recognized in both surface water and sediment samples (Fig. 6B). Moreover, the abundance of MGEs in the surface water surpassed that in the sediment, which was consistent with ARGs abundance. Previous investigations have also underscored the significant role of MGEs in shaping ARG abundance [26]. The abundance of MGEs was highly associated with the total abundance of ARGs, suggesting their utility as potential indicators for quantitative estimations of the resistome contamination [57]. On the one hand, microorganisms and antibiotics can indirectly affect the spatiotemporal distribution of ARGs mainly through MGEs [50]. On the other hand, stochastic mechanisms mediated by MGEs had a higher contribution to ARG assemblages than other processes [58].
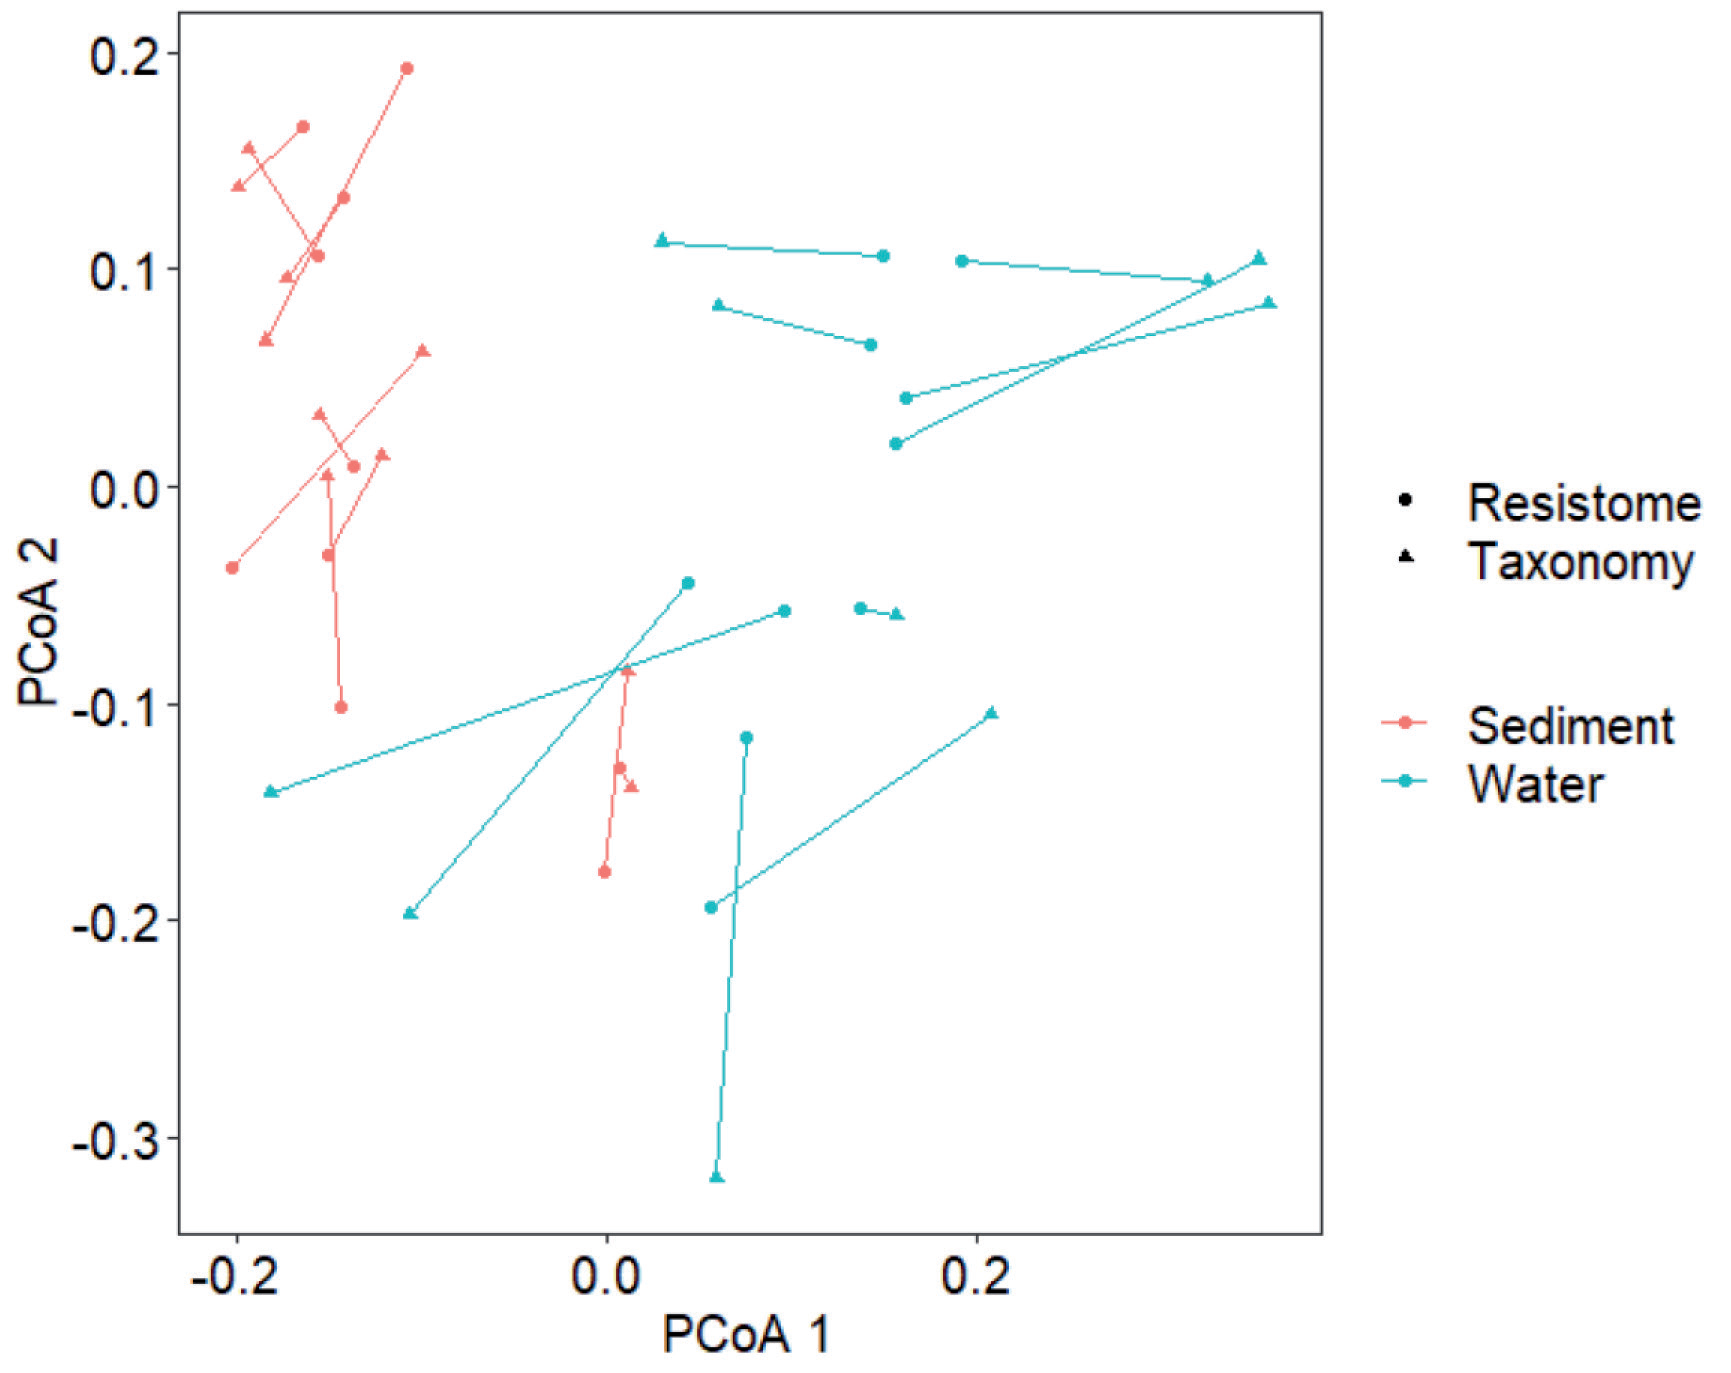
Fig. 6.
The relative abundance of ARGs in sediment and water samples (A); The relative abundance of MGEs in sediment and water samples (B)
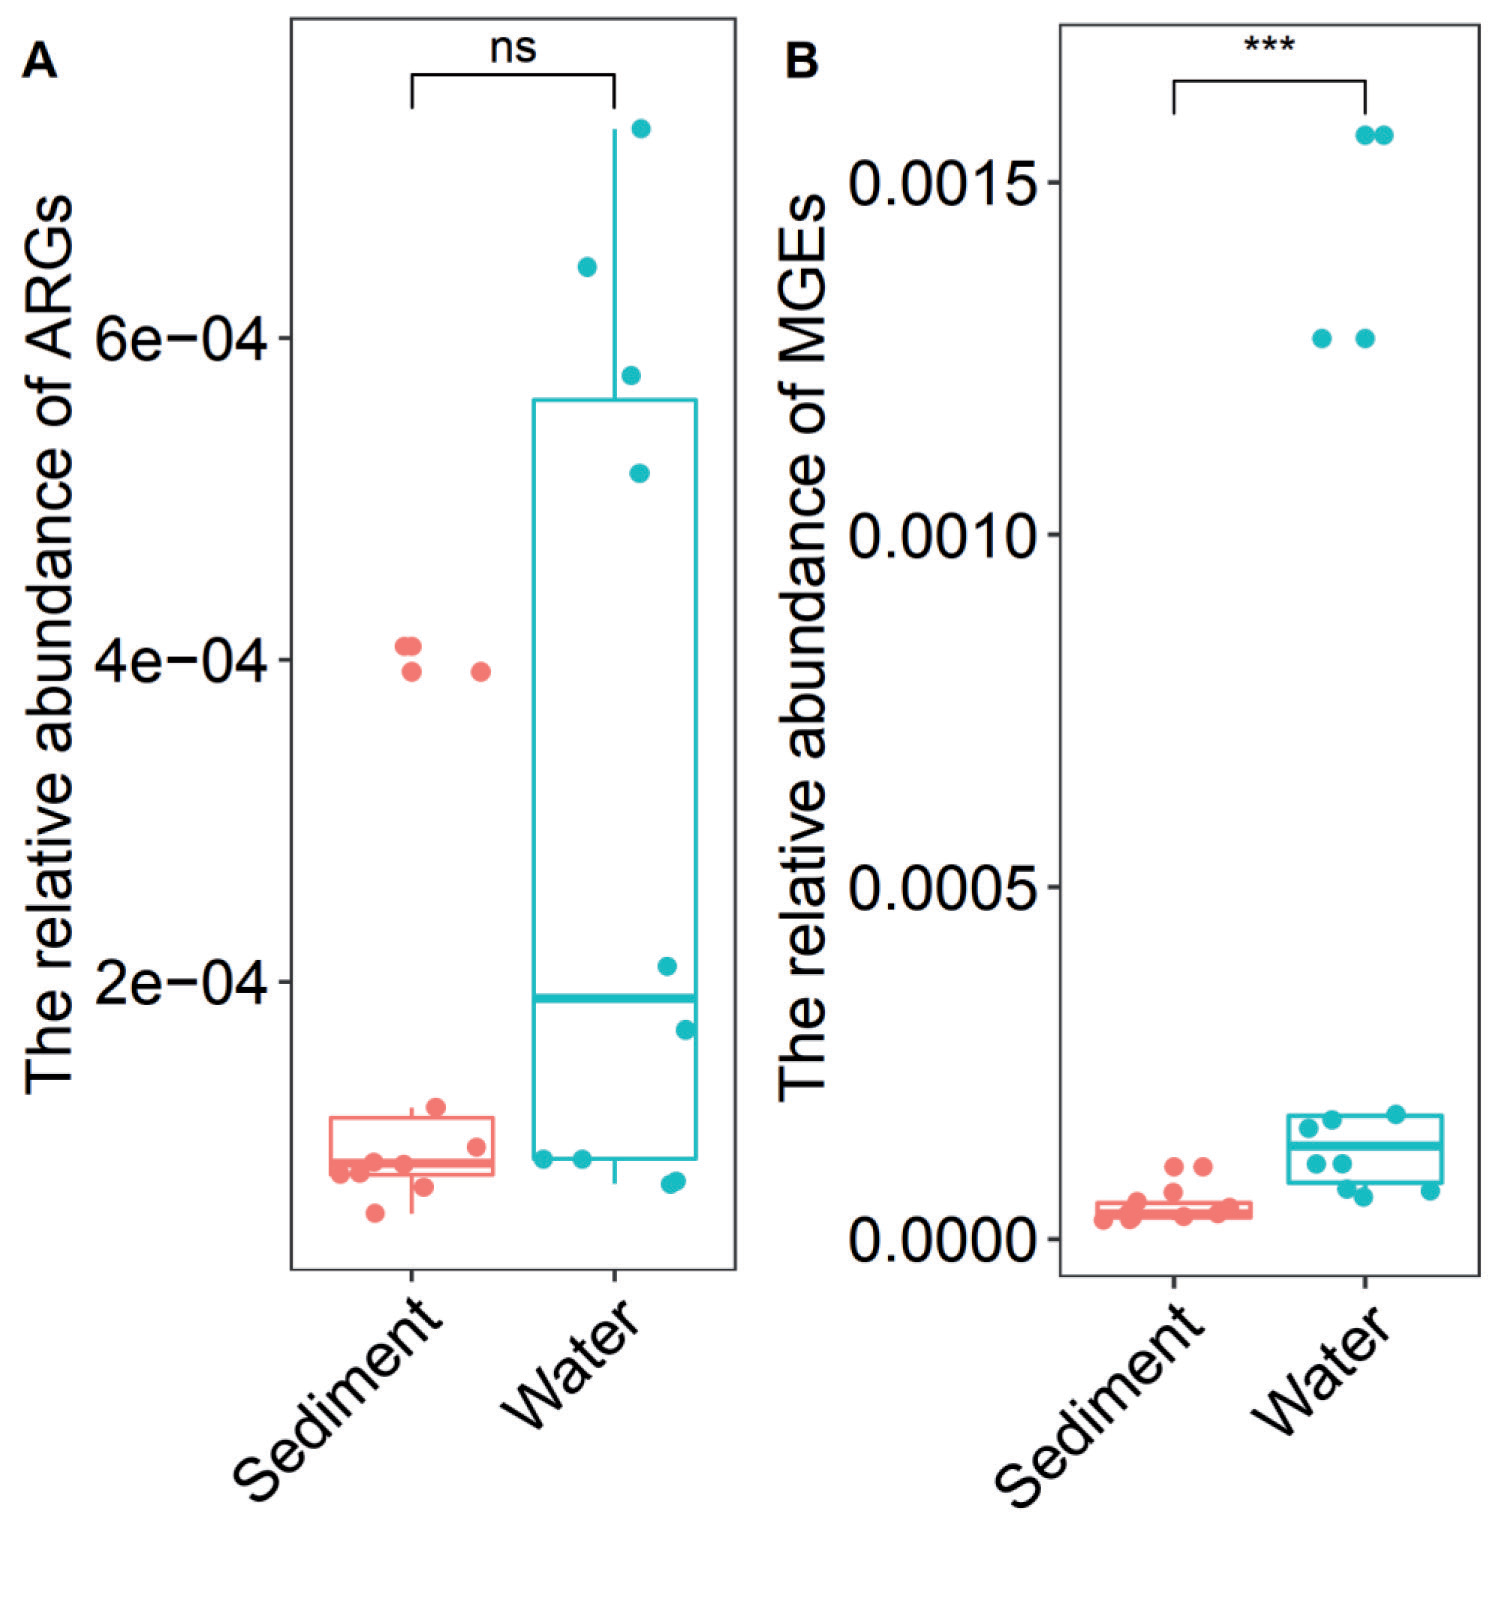
Szekeres et al. (2018) emphasized the role of MGEs in maintaining and augmenting associated resistance phenotypes [29]. The study suggests that microbes bearing MGEs can adapt to selective pressures exerted by different categories of antibiotics [59]. As a case, Yu et al. (2022) identified MGEs as the primary determinant of ARG propagation in the Yellow River [60]. A higher abundance of MGEs, especially plasmid, increased the potential ARG dissemination risk, because most of the resistance mechanisms were carried by MGEs that can be transferred through horizontal gene [61]. In our present research, we identified a higher prevalence of MGEs in surface water samples compared to sediment samples from Poyang Lake, mirroring the ARG distribution across these samples. Multidrug was the most prevalent gene in the surface water samples. This study demonstrated that multidrug and sulfonamide resistance genes had a greater potential to transfer because they were more frequently carried by MGEs [61]. Thus, curtailing the spread of ARGs becomes a crucial aspect of ensuring the biosafety of drinking water, and, consequently, human health.
Conclusions
ARGs pose a mounting global threat, endangering the progress of modern medicine and presenting a grave health risk to the populace. This study focused on the distribution of ARGs in Poyang Lake and the key impact factors. The findings revealed a wide variety of ARGs present in both surface water and sediment samples, denoting their prevalence in the studied region. Notably, the surface water displayed higher ARG abundances than the sediment, thus implying a greater potential for ARG spread within the lake. The abundance of ARGs across extensive geographical areas was found to correlate with localized human activities. Additionally, the microbial abundance and MGEs appeared to significantly affect the ARG distribution. By providing evidence of the prevalence of ARGs in both surface water and sediment, this study paves the way for future investigations to elucidate the interplay between these two matrices and their effect on ARG dissemination in Poyang Lake. It is anticipated that these research efforts will enhance our understanding of how human activities influence the genesis and propagation of ARGs in lake environments.

