

Introduction
Zanthoxylum armatum DC. (Rutaceae) is a globally recognized edible medicinal plant. It is characterized by strong adaptability, wide distribution and convenient management, and has good economic benefits [1-2]. Climate has a great influence on leaf micromorphology and leaf rust resistance [3-6]. Leaf rust, caused by Coleosporium zarathoxyli, is one of the most important leaf diseases of Z. armatum. It is highly contagious, with a disease rate of 30%-60% in susceptible areas and more than 80% in severely diseased areas. The large-scale defoliation of susceptible plants and the sharp decrease in yield caused by C. zarathoxyli have seriously restricted the industrial development of Z. armatum [5].
Hormones play an important role in plant growth and development and stress resistance, and salicylic acid (SA) is an important defensive hormone and endogenous elicitor that mediates the signal transduction system, and it can stimulate both localized acquired resistance (LAR) and systemic acquired resistance (SAR) [7, 8]. After induced by exogenous substance SA, plants will produce induced resistance, and a series of signal transduction and material metabolism changes will occur in the body, such as oxidative burst, antibacterial protein, endogenous SA accumulation; changes of CAT, POD, PPO, PAL activities related to active oxygen or resistance; plant antitoxins, and deposition of lignin, cork and callose; and the transcriptional expression of defense signaling pathways and pathogenesis-related (PR) genes; there are other non-enzymatic active substances such as soluble sugar, proline, soluble protein and so on [9, 10].
PRs, SAR marker genes closely related to plant disease resistance, play an important role in plant defense systems [11]. The PRs currently isolated are grouped into 17 families, PR1 to PR17, which typically encode antimicrobial proteins, nucleases, chitinases, and others [12]. Some PRs participate in plant defenses against rust [13]. Pathogenesis-related protein genes, such as TaLr19PR1, TaLr35PR2, TaLr35PR5, and TaPR10, contribute to wheat defense against rust [14- 17]. Jing et al. [18] found that the expression level of PR5 was elevated and the resistance of sunflower to leaf rust was enhanced after oligosaccharide induction. The purified protein expressed by the PmPR10-3.1 gene in white pine inhibited the mycelial growth of Cronartium ribicola A. Dietr. in vitro [19].
The PR gene plays an important regulatory role in the plant rust resistance and defense response, but the Z. armatum PR gene has not yet been reported. Previously, we screened the PR gene ZaPR4b, which may be related to the resistance of green pepper to leaf rust, by comparative transcriptome analysis of the disease-resistant and susceptible varieties. In this study, we cloned ZaPR4b from Z. armatum, and conducted bioinformatics, subcellular localization, and expression pattern analyses to provide a reference gene for further studying the defense mechanism of Z. armatum against leaf rust.
Material and Methods
Plant Materials
We collected, Jiuyeqing (JYQ), the main cultivar grown in Chongqing, China (selected from the varieties of Z. armatum in Jiangjin, Chongqing, and approved by the Chongqing Forest Variety Committee in 2004), and four wild resource varieties resistant to leaf rust (Yeqing pepper (YQP), Chuanqiongwuci (CQWC), Pingjiangqing (PJQ), and Smal leaf pepper (SLP)) from the germplasm resource nursery of Z. armatum at Chongqing University of Arts and Sciences, Yongchuan District, Chongqing, China (29°20′N, 105°43′ E).
Total RNA Extraction and Gene Cloning
According to the manufacturer’s instructions, we extracted the total RNA from the leaf tissues of Z. armatum using a universal plant RNA extraction kit (Beijing Huayueyang), and we determined RNA integrity by 1% agarose gel electrophoresis. We obtained the cDNA product by reverse transcription using HiScript® II 1st Strand cDNA Synthesis Kit reagent (Vazyme, Nanjing, China) according to the instructions, which we stored in an ultra-low-temperature refrigerator at –80ºC after packaging.
Based on the transcriptome data, we mined the ZaPR4b gene sequence, and designed and synthesized the primers (Table 1). The full-length open reading frame of ZaPR4b were amplified using TaKaRa high-fidelity DNA polymerase Prime-STAR HS DNA Polymerase using the cDNA of Z. armatum leaves as a template. The total amplification volume was 50 µL: 10 µL cDNA template + 2 µL primer + 2 µL primer + 25 µL enzyme reaction solution + 11 µL ddH2O. The PCR amplification procedure was as follows: predenaturation, 94ºC, 5 min; 30 cycles of denaturation, 94ºC, 30 s; annealing, 53ºC, 30 s; extension, 72ºC, 30 s; and end extension, 72ºC, 5 min, 4ºC, 10 min. We detected the PCR products using 1% agarose gel electrophoresis at 180 V. The PCR products were recovered using an agarose gel recovery kit (DP209; Tiangen, Beijing, China). We ligated the PCR product into the pMD19-T vector and transformed into Escherichia coli DH5α cells. We selected and sent positive monoclonal bacteria to Tsingke Biotechnology Co., Ltd. for sequencing.
Bioinformatics Analysis
We performed homology analysis using the NCBI NCBI-BLAST program (https://blast.ncbi. nlm.nih.gov/Blast.cgi?PROGRAM=blastn&PAGE_ TYPE=BlastSearch&LINK_LOC=blasthome).
Table 1.
Primers used in this study.
We used NCBI ORF Finder program (http://www. bioinformatics.org/ sms/orf_find.html) to search for the open reading frames. We obtained the amino acid sequence using EditSeq software, and we performed multiple sequence alignments using DNAMAN (2.6) software. We analyzed a variety of physical properties and biochemical parameters (such as protein molecular weight, pI, hydrophilicity, etc.) in the amino acid sequence using the ProtParam database (https://web.expasy.org/protparam/). We used online software NetNGlyc 1.0 (http:/www.cbs.dtu.dk/services/ NetNGlyc), NetPhos 3.1 (http://www.cbs.dtu.dk/ services/NetPhos), SignalP 4.1 (http://www.cbs.dtu.dk/ services/SignalP-4.1), SOPMA (https://npsa- prabi.ibcp. fr/cgi-bin/npsa_automat.pl?Page=npsa_sopma.html), and SWISS-MODEL (https:// swissmodel.expasy.org/) for protein glycosylation sites, phosphorylation sites and protein kinase binding sites, and signal peptides and amino acid secondary and tertiary structure prediction. We constructed the phylogenetic tree of amino acid sequence with MEGA (6.06) software.
Subcellular Localization
The full-length CDS sequence of ZaPR4 was cloned into the pA7-GFP vector to generate the 2*35S::ZaPR4-GFP cassette. The entire 2*35S::ZaPR4-GFP cassette was then inserted into the PHB vector for tobacco leaf epidermis cell transformation. The GFP signals was visualized with a confocal scanning microscope (Nikon A1, Kanagawa, Japan) at 72 h after infiltration.
SA-Induced Resistance and Leaf Rust Resistance aAnalyses of Different Green Pepper Varieties
In February 2021, JYQ and four other wild resources were young plants, which we allowed to grow for approximately one year. We then selected ten plants of each variety with strong growth and no pests or diseases. According to the method of Zheng et al. [20], we separately inoculated the plants with C. zarathoxyli at a concentration of 105 spore·mL-1, and then we investigated the resulting infection. We used the resistance standard of wheat stripe rust grade 0-4 as a reference [21], and we determined the resistance of different Z. armatum varieties to leaf rust at the seedling stage, which was repeated three times.
In July 2021, we sprayed different concentrations (0.25, 0.50, 1.00, 2.00, and 4.00 mM) of SA solution on the leaves of JYQ plants, with the same amount of distilled water applied as the control with nine plants in each treatment, with three replicates per treatment. After treatment, we placed the plants in a moisturizing bucket at 20±2ºC for 12 h in dark and inoculated them according to the method of Zheng et al. [13] after 2 days of inducer treatment. Ten days after inoculation, we used Hu’s [21] grading standard to investigate the incidence and calculate the disease index. We calculated the induced resistance effect as the percentage decrease in the disease index [22]: induced resistance effect (%) = 100 × (control disease index - treatment disease index) / control disease index.
Quantitative PCR for Expression Analysis
In April 2021, we inoculated JYQ and four wild resource varieties with the sheath rust fungus. When the leaves of JYQ were approximately 50% covered with diseased spots, we separately collected four leaves of each variety to remove the rust spots on the surface of the leaves. This was repeated three times. In August 2021, with distilled water as the control, we treated the leaves of JYQ with 1 mM exogenous SA with the highest concentration of induced resistance for 2 days, and then inoculated the plants with sheath rust. We collected the leaves of JYQ at 2, 4, 6, 8, and 10 days after inoculation, with four leaves per treatment and three replicates. In May 2022, we randomly selected three healthy and disease-free JYQ plants to collect root, stem, leaf, and fruit samples. We repeated the experiment 3 times.
We sealed the collected samples in a bag, which we then quickly froze in liquid nitrogen, and stored at –80ºC. We used quantitative PCR (qPCR) to study the expression of ZaPR4b in different tissues, SA-induced leaves, and the leaves of different resistant varieties. We generated fluorescent quantitation primers (Table 1) using the online software Primer-BLAST (https://www.ncbi.nlm.nih. gov/tools/primer-blast/ index.cgi?LINK_ LOC=BlastHome). We selected ZaUBC as the reference gene, and we performed the chemical reaction of fluorescence quantitative PCR in a StepOnePlus according to the fluorescence quantitative PCR instructions (Jena, Germany). We divided each tissue sample into 4 groups. The specific reaction process was: 95ºC for 30 s; 95ºC for 5 s, and 60ºC for 30 s, from denaturation to extension, we used a total of 40 cycles; the end conditions (melting curve) were: 95ºC for 15 s, 60ºC for 1 min, and 95ºC for 15 s. After the completion of the reaction, we processed and analyzed the data using the 2-∆∆CT method [23].
Results
Cloning and Sequence Analysis of ZaPR4b in Z. armatum
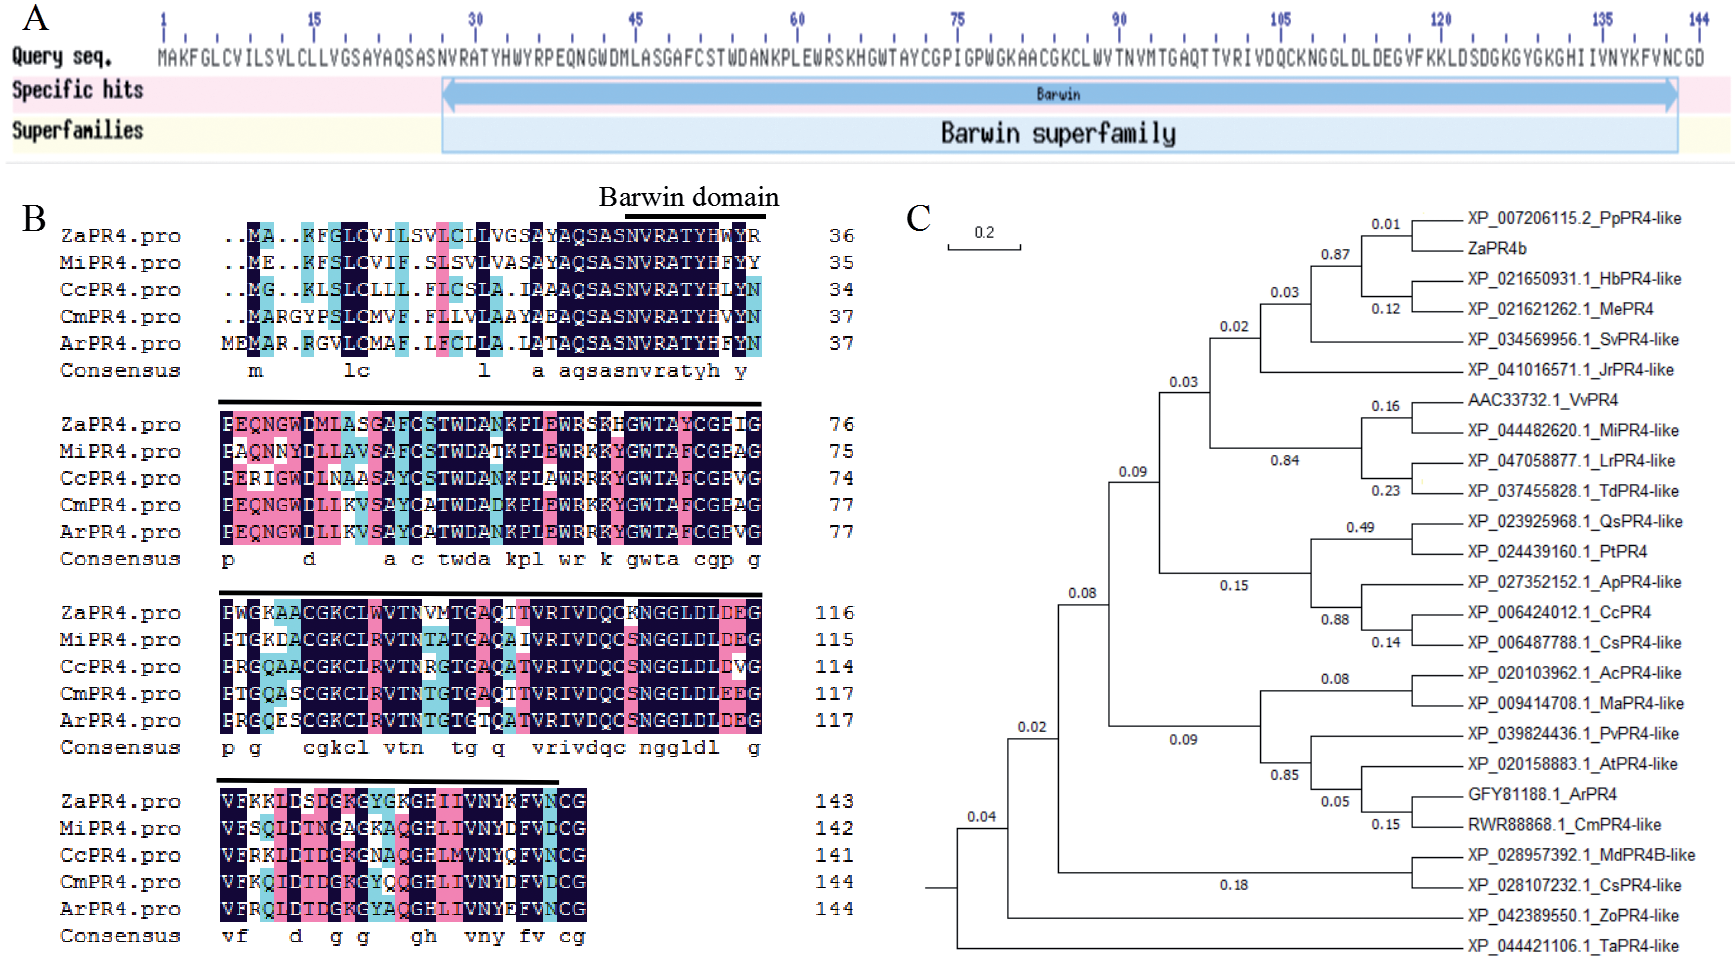
According to RNA-seq data, we identified a PR-annotated gene (>cb12747_c9/f1p0/723) that may be related to disease resistance and designed primers based on the sequence information. We obtained bands of 736 bp (full gene length) and 435 bp (full CDS length) (Fig. 1a), using PCR amplification. Through monoclonal sequencing, we obtained the CDS sequence of the PR gene. NCBI ORF Finder analysis showed that the open reading frame of the PR gene sequence is 435 bp, and the number of encoded amino acids is 144 (Fig. 1b). We used the NCBI CDD database to analyze the amino acid sequence of PR, and found that the C-terminus of the PR protein contains a classic Barwin conserved domain, distributed in the 27-142 amino acid interval (Fig. 2a). At the same time, we found the PR protein does not contain a chitin-binding domain which belongs to the typical structure of class II PR4. Therefore, we named the PR gene of Z. armatum ZaPR4b.
Bioinformatics Analysis of ZaPR4b in Z. armatum
Using the NCBI BLASTP database, we found that ZaPR4b has high homology with MiPR4 (Mangifera indica, XP_044482620.1), CcPR4 (Citrus clementina, XP_006424012.1), ArPR4 (Actinidia rufa, GFY81188.1), and CmPR4 (Cinnamomum micranthum, RWR88868.1). The sequence similarities are 72.92%, 70.83%, 69.18%, and 69.18%, respectively (Fig. 2b). Using MEGA 6.06, We analyzed the genetic relationship between the amino acid sequence encoded by the ZaPR4b gene and PR4 amino acid sequence of 24 related plants, such as citrus and peach. The results (Fig. 2c) showed that ZaPR4b has a close genetic relationship with the PR4 of peach (PpPR4), rubber tree (HbPR4), and cassava (MePR4), but a distant genetic relationship with the PR4 of Clemens puppy (CcPR4), kiwi (ArPR4), and camphor (CmPR4).
Using the ProtParam database, we predicted the theoretical pI of the ZaPR4b protein is 8.62; its relative molecular mass is 15747.07; the amount of Gly in the amino acid sequence is the largest, accounting for 12.5%; and the molecular formula of the protein is C704H1071N191O199S11. The stability index (II) value of the protein is 17.23, which indicates a stable protein. The hydrophilic range of the protein is far beyond the hydrophobic range, and the average hydrophilic rate is –0.122, which indicates a hydrophilic protein.
Fig. 1.
Cloning of ZaPR4b gene and CDS, amino acid sequence. a) M, marker; 1, mixed PCR product of DNA and cDNA amplification; 2, full-length PCR product of gene; 3, CDS amplification product of the gene. b) Box, start/stop codon; solid line below, characteristic sequence of ZaPR4b amino acid sequence; dotted line below, binding domain of Barwin; curve, poly A tail.
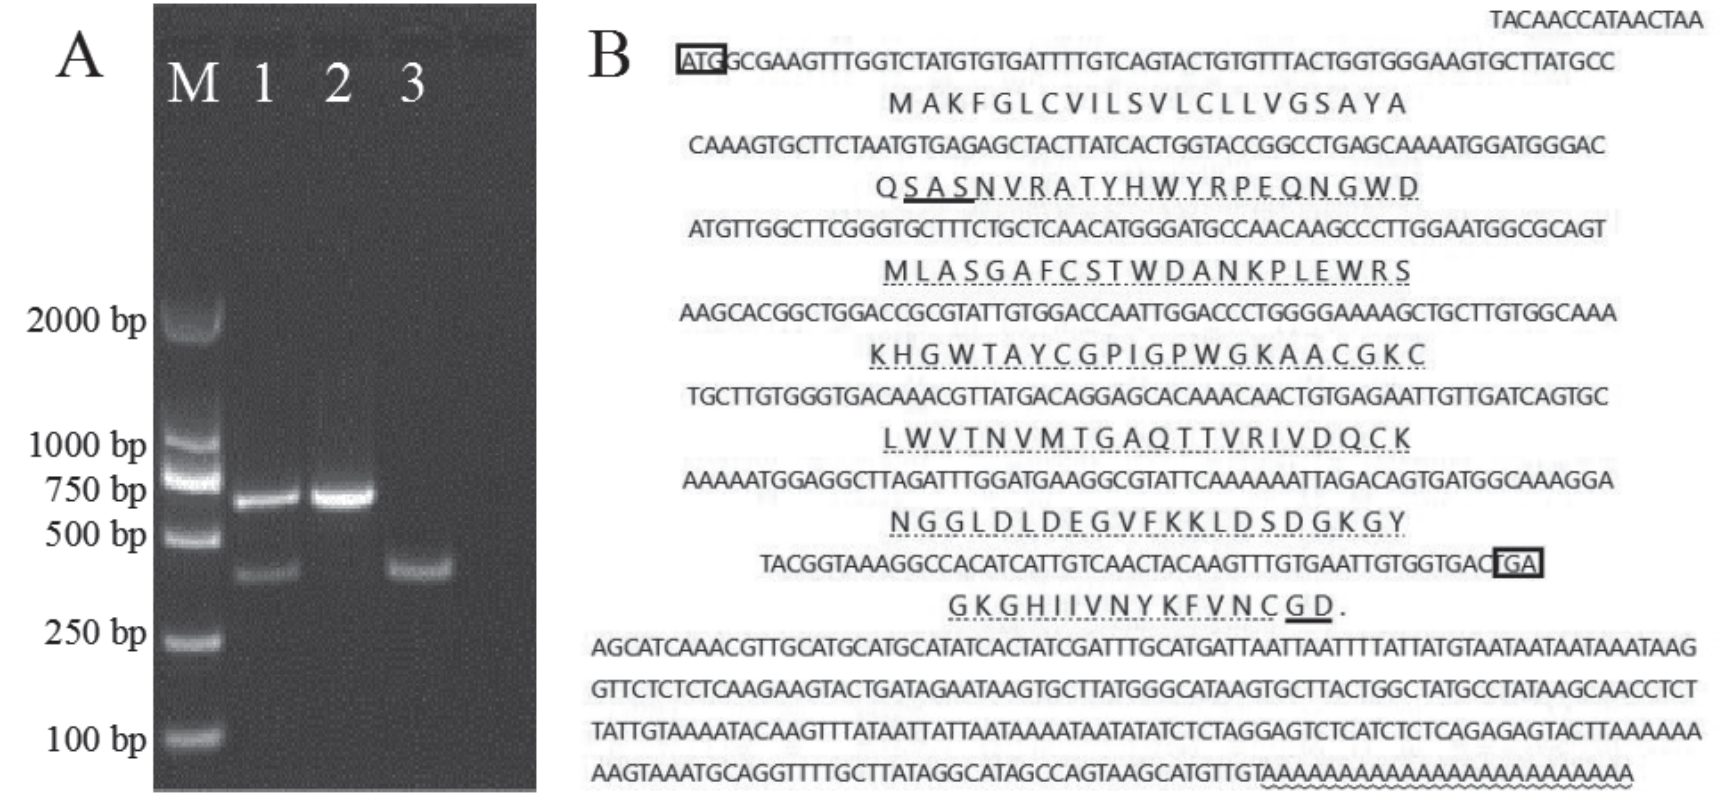
Fig. 2.
Bioinformatics analysis of ZaPR4b gene. a) Conserved domain prediction of ZaPR4b; b) ZaPR4b amino acid sequence homology comparison; c) phylogenetic tree of ZaPR4b and PR4 proteins of 24 other species.
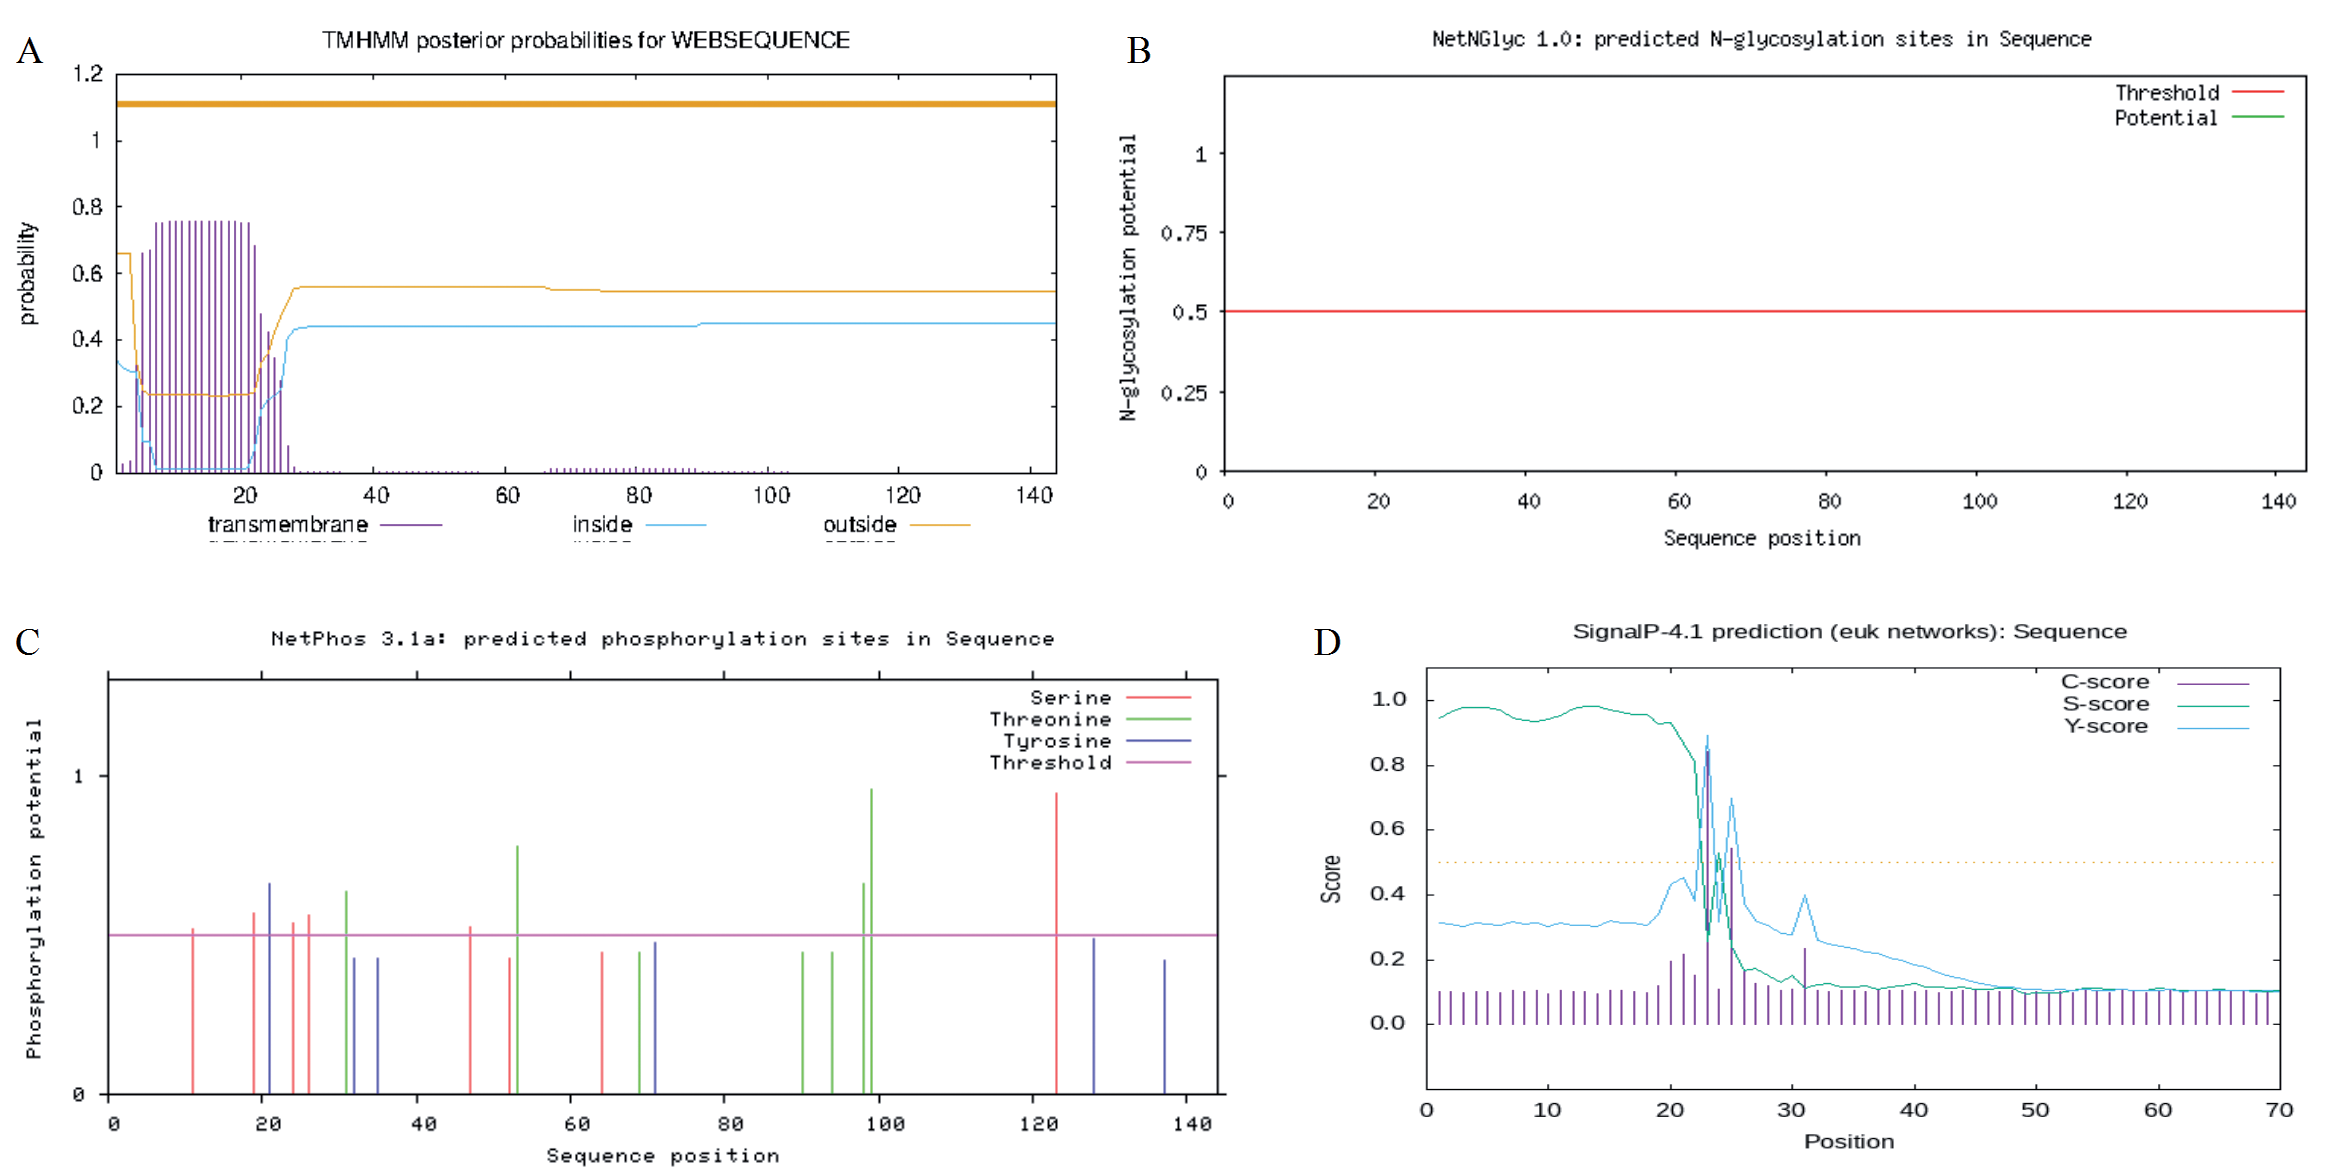
The transmembrane domain of the ZaPR4b protein predicted by TMHMM Sever v2.0 showed that the whole ZaPR4b sequence is outside the membrane, without a transmembrane helix region, and does not belong to the transmembrane protein (Fig. 3a). The online software NetNGlyc 1.0 predicted the glycosylation site of ZaPR4b protein and showed that the protein does not contain glycosylation sites (Fig. 3b). We used NetPhos 3.1 to predict the phosphorylation sites and protein kinase binding sites of ZaPR4b. We found eleven phosphorylation sites when the predicted value was greater than 0.5, including six serine sites, four threonine sites, and one tyrosine site (Fig. 3c). We predicted the signal peptide of the ZaPR4b protein using SignalP 4.1, and found that the ZaPR4b contains one signal peptide site and is a secretory protein according to the C, S, and Y values (Fig. 3d).
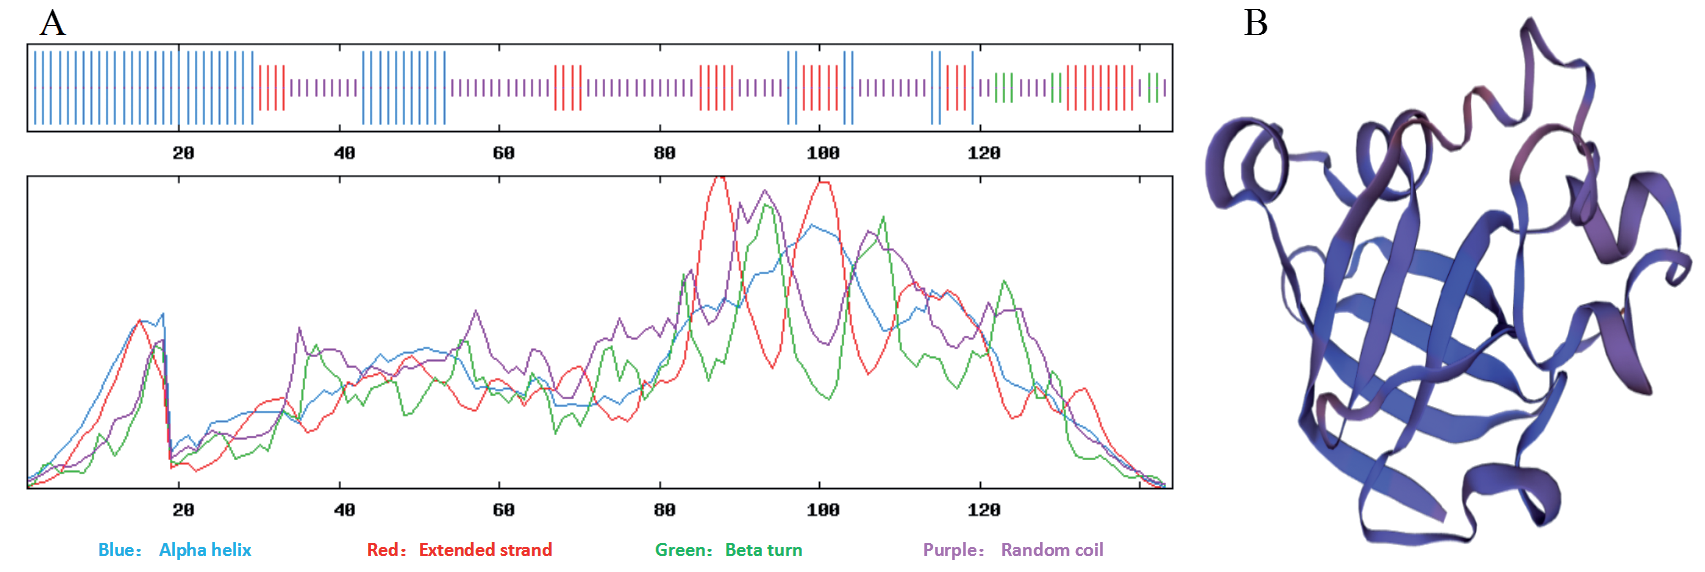
We predicted the secondary structure of the amino acids encoded by ZaPR4b using the SOPMA database. The results showed that. the molecular structure of the ZaPR4b protein is dominated by random coils (59, accounting for 40.97%) and α-helix structures (48, accounting for 33.33%), whereas the extended chain (30, accounting for 20.83%) and a small amount of β sheets (7, 4.86%) are dispersed in it (Fig. 4a). We used SWISS-MODEL online software to model the tertiary structure of ZaPR4b. With 4jp6.1.A papaya Barwin-like protein as a template, we used 23-144 amino acid residues used to establish the model: the coverage was 84.72%, the sequence consistency was 72.13%, and the sequence similarity was 60.42% (Fig. 4b).
Subcellular Localization of ZaPR4b
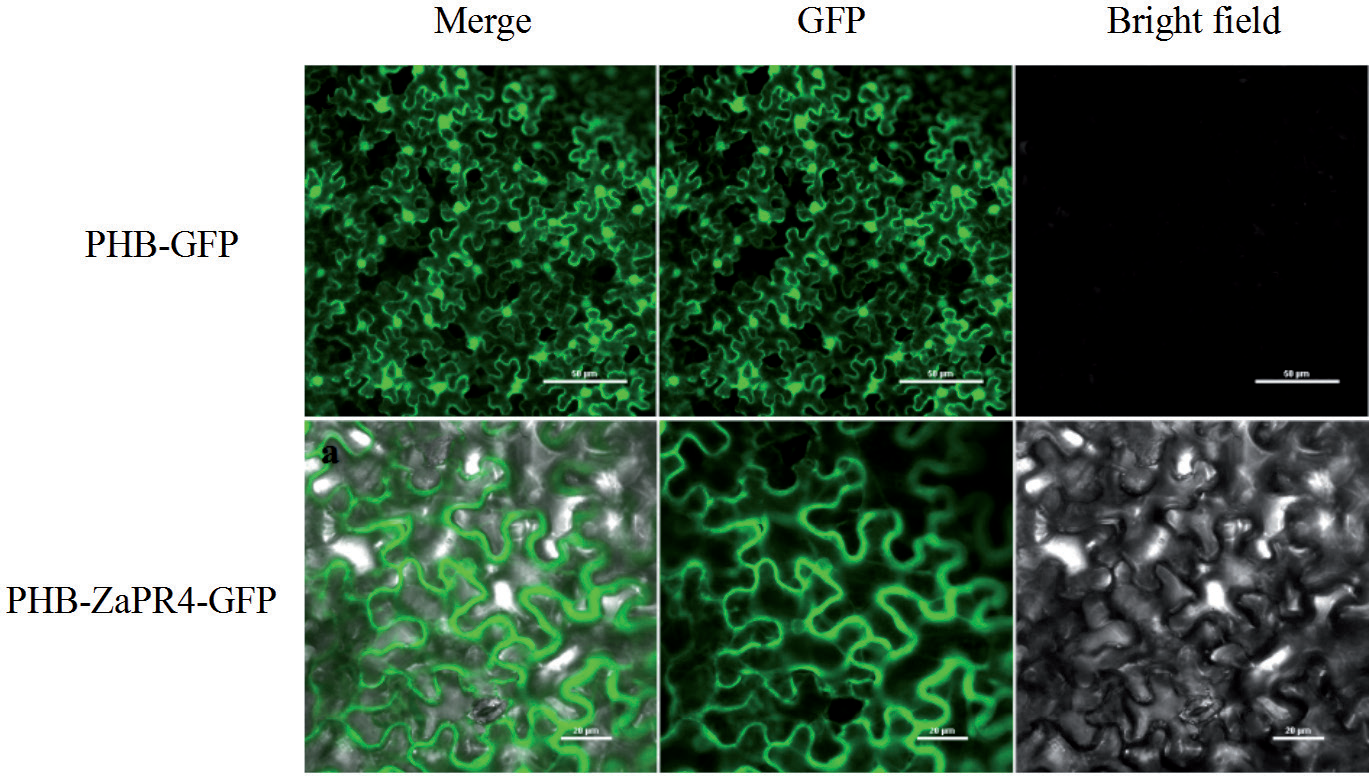
To verify the accuracy of ZaPR4b localization prediction, we performed subcellular localization. The results showed that the fluorescence signals of ZaPR4 were partially overlapped with plasma membrane in tobacco epidermal cells (Fig. 5), suggesting the preferential membrane location. Interestingly, ZaPR4 was also detected in the cytoplasm and nuclear membrane.
Expression Analysis of ZaPR4b in Different JYQ Tissues and Different Leaf-Rust-Resistant Varieties
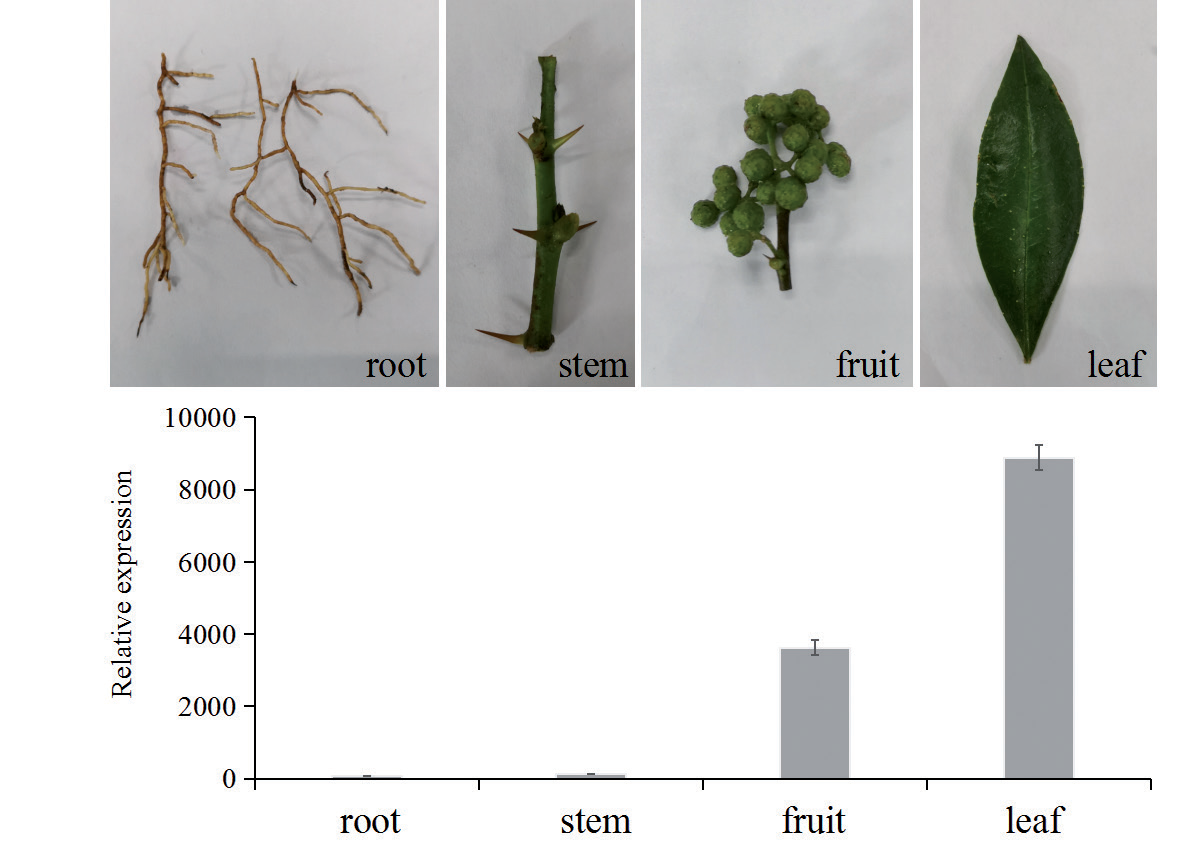
We analyzed the expression of ZaPR4b in different tissues of JYQ using qPCR. The results showed that ZaPR4b expression was tissue-specific (Fig. 6) which is mainly expressed in the leaves and fruits, less in the roots and stems, and the most in the leaves.
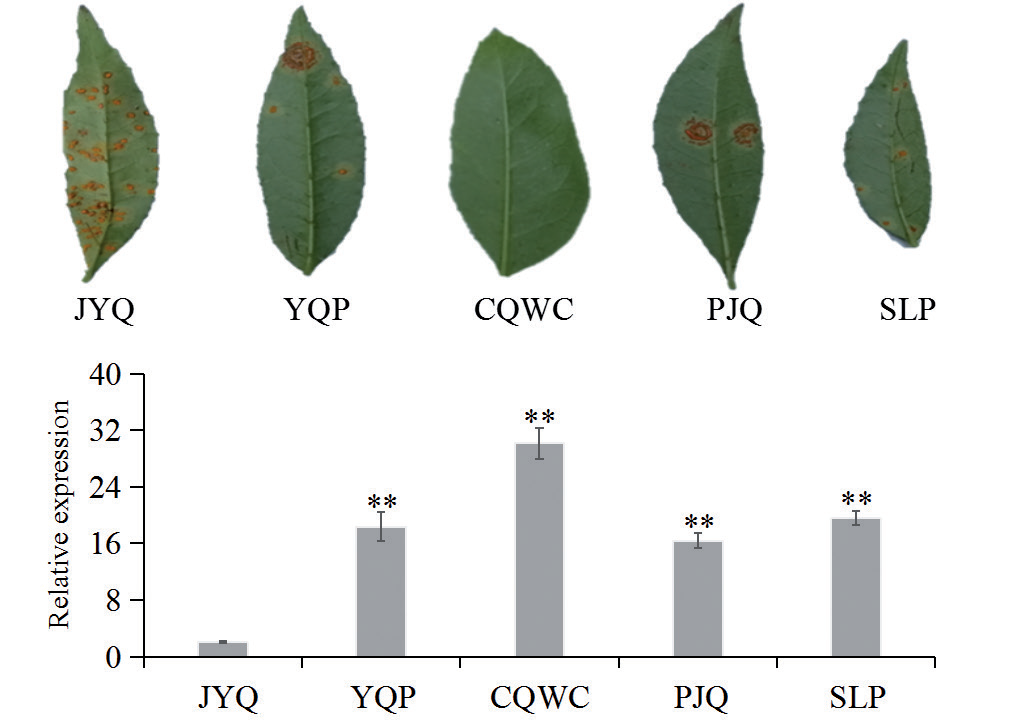
We identified the leaf rust resistance of JYQ and four rust-resistant wild resources in the field and found that these different varieties showing different levels of resistance to C. zarathoxyli, the lesions on CQWC (medium resistance) covered less than 5% of the leaf area, indicating this variety is highly resistant to leaf rust. YQP, PJQ, and SLP (medium resistance) were moderately resistant to leaf rust, whereas the lesions on JYQ (sensitive) plants accounted for about 50% or more of the leaf area, indicating this variety is sensitive to leaf rust (Fig. 7, Table 2). We analyzed the expression of ZaPR4b gene in different leaf rust-resistant varieties when the JYQ leaves were 50% covered with lesions and found that ZaPR4b’s expression were positively correlated with the resistance of the tested varieties (Fig. 7).
Fig. 3.
Prediction analysis of ZaPR4b. a) Transmembrane structure prediction; b) glycosylation site prediction; c) phosphorylation site and protein kinase binding site prediction; d) signal peptide site prediction.
Expression Analysis of ZaPR4b Induced by SA in JYQ
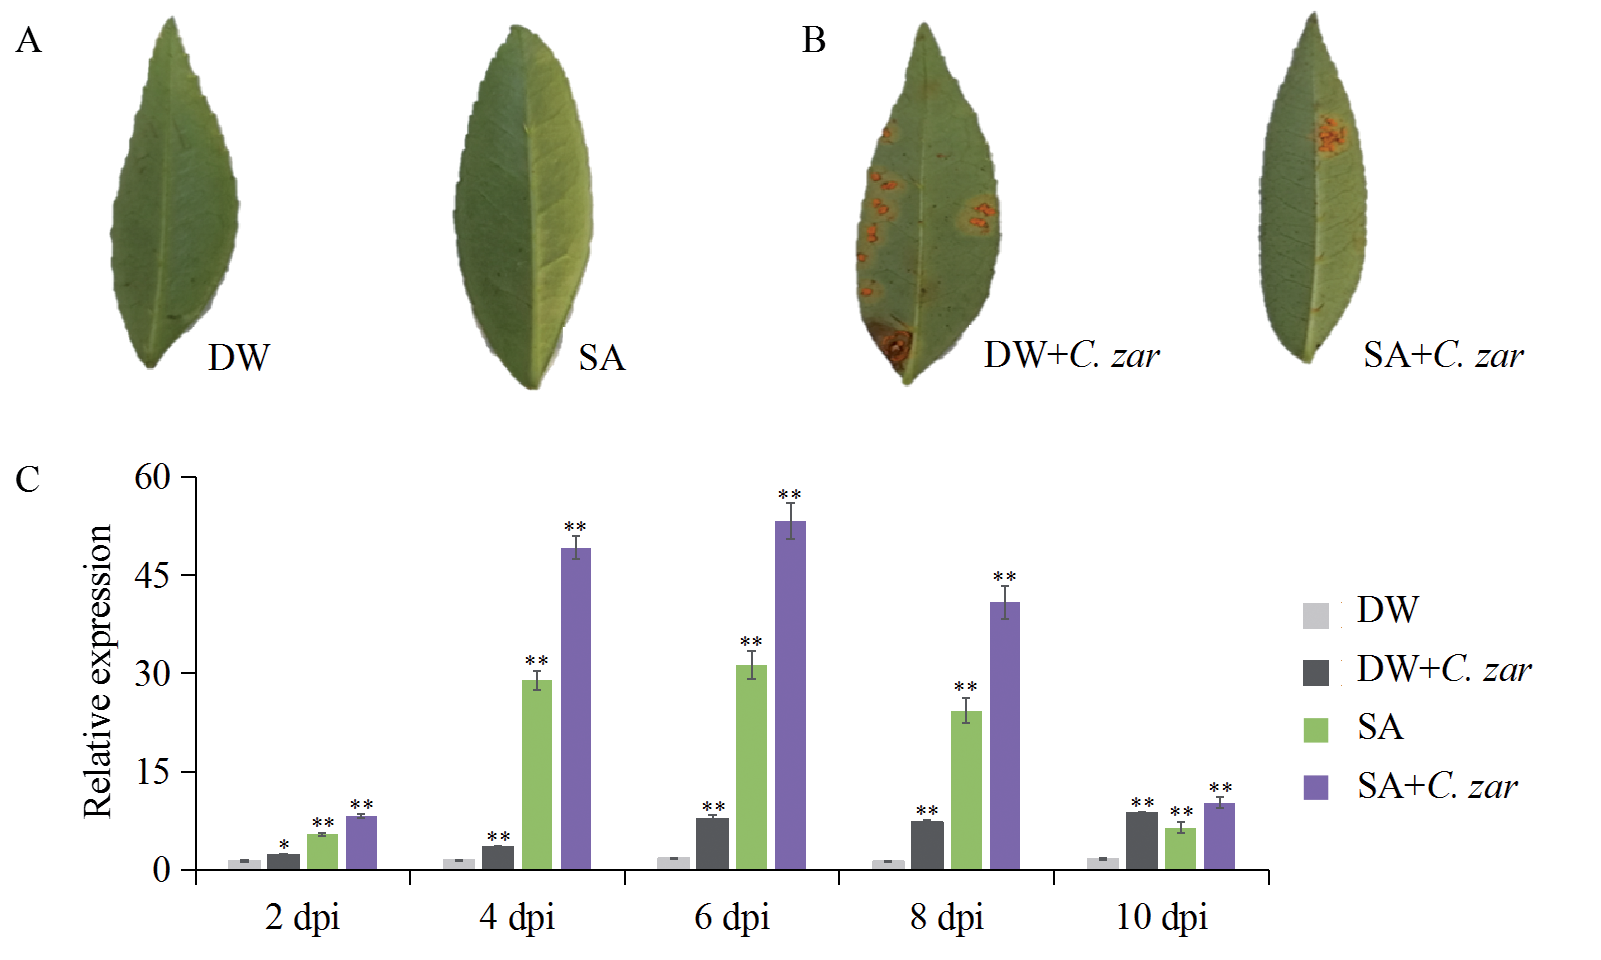
PRs are systemic acquired resistance marker genes that are closely related to plant disease resistance in the SA signal transduction pathway. To study the induction effect of SA on the ZaPR4b gene in Z. armatum, we inoculated the leaf-rust-sensitive variety JYQ with C. zarathoxyli after SA induction. The results showed that low concentrations of SA had no obvious inhibitory effect on the leaf rust, whereas high concentrations of SA damaged the seedlings. After 0.5-1 mM SA treatment and inoculation of C. zarathoxyli urediospores, the resistance of C. zarathoxyli to leaf rust substantially improved, the induction effect reached 55.04%, and no harmful to the seedlings. (Table 3).
We detected the expression level of ZaPR4b in JYQ leaves at different time points after pretreatment with 1 mM exogenous SA and inoculation with C. zarathoxyli. The results showed that the expression of the ZaPR4b gene in leaves treated with DW and then inoculated with C. zarathoxyli (DW + C. zar), only treated with SA (SA) or treated with SA, and then inoculated with C. zarathoxyli (SA + C. zar) were notably increased compared with the control (DW) treatment. The expression level of ZaPR4b in the leaves treated with SA (SA) and treated with SA, and then inoculated with C. zarathoxyli (SA + C. zar) were considerably higher than that in leaves treated with DW and then inoculated with C. zarathoxyli (DW + C. zar) (Fig. 8).
Table 2.
Evaluation of leaf rust resistance of Zanthoxylum armatum varieties.
| Symbol | Varieties | Identification standards | Resistance level |
|---|---|---|---|
| JYQ | Jiuyeqing | 3 | MS |
| YQP | Yeqing pepper | 2 | MR |
| CQWC | Chuanqiongwuci | 0 (1) | HR |
| PJQ | Pingjiangqing | 2 | MR |
| SLP | Small leaf pepper | 2 | MR |
Table 3.
Resistance to leaf rust induced by different concentrations of SA.
Discussion
PR proteins are ubiquitous in most higher plants and play important roles in many physiological processes, such as plant growth and development, and the stress response. PR genes have been successfully cloned in a variety of plants and exist in the form of gene families, which are classified into 17 families of PR1-PR17 [12]. In this study, the results of BLAST amino acid sequence alignment of the ZaPR4b gene showed that it is homologous to the PR4 protein of mango, citrus, and kiwifruit, belonging to the PR4 family. PR4 proteins are divided into two categories according to whether they have a chitin-binding domain (CBD). Class I PR4 proteins contain CBD, such as tomato-injury-inducing protein [24]. Class II PR4 proteins, such as grape downy mildew resistance-related proteins VpPR4b and VvPR4b, have a signal peptide at the N-terminus, a classical Barwin conserved domain at the C-terminus, and no chitin-binding domains; they are located on the membrane [25]. We found that the C-terminus of the ZaPR4b protein contains a Barwin domain and does not contain a chitin-binding domain, belongs to class II PR4 and was locateded on plasma and nuclear membrane.Plant PR genes have tissue-specific expression characteristics; they can be induced by a variety of biotic and abiotic stresses [26-28], and they participate in the plant defense response process induced by diseases and insects [29-30]. The relative expression level of the VvPR1 gene is the highest in grape leaves [31]. The expression level of CsPR5 is the highest in the stem and leaf tissues of tea plants, and it is slightly expressed in the flowers, seeds, and roots [32]. The results showed that the expression level of ZaPR4b substantially differs among the four tissues, with the highest expression level in the leaves and the lowest expression level in the roots and stems. The high expression level of ZaPR4b in the leaves indicates that it plays an important role in protecting Z. armatum against pathogens and pests. Similar studies reported that banana MaTLP1 is mainly expressed in the roots, which are the main sites of Fusarium wilt infection [33]. The expression level of AsPR5 in garlic is the highest in the stem, which is the main site of Fusarium oxysporum f. sp. cepae (FOC) infection. Fusarium oxysporum infection can induce considerable upregulation of the expression of the AsPR5 gene in the stem, which indicates that this gene might be involved in the defense process of garlic against Fusarium oxysporum [28]. The results of this study showed that ZaPR4b expression in Z. armatum leaves is substantially upregulated after leaf rust infection, indicating that ZaPR4b may be involved in the defense against leaf rust.
Plant SAR is a defense mechanism that induces plants to continuously resist pathogenic microorganisms. SAR requires the participation of the SA signal molecule and is related to the accumulation of PRs [13, 34]. The expression level of the PR gene is closely related to the interaction between the host plant and pathogen. Overexpression of PR1 in tobacco can enhance its resistance to Sclerotinia sclerotiorum, whereas overexpression of NtPR1a can improve the resistance of tobacco to Fusarium wilt [35, 36]. Overexpression of GmPR10 in soybeans can enhance the resistance of transgenic plants to Pseudomonas sojae [37]. Rathod et al. [38] found that PR1 expression level in peanuts was significantly higher in rust-resistant varieties than in susceptible varieties. The results showed that SA remarkably increased the expression level of ZaPR4b gene in leaves of JYQ plants and its resistance to leaf rust. The results of qPCR analysis showed that the expression of the ZaPR4b gene is positively correlated with the resistance of the tested varieties, suggesting that the ZaPR4b gene may play an important role in the resistance of Z. armatum to leaf rust through positive regulation, but further experiments are needed. At present, we are constructing a genetic transformation system of Z. armatum to provide a theoretical basis for clarifying the function and mechanism of ZaPR4b against leaf rust in Z. armatum.
Conclusions
In this study, we cloned ZaPR4b from JYQ, a leaf-rust-susceptible variety of Z. armatum. Sequence analysis results showed that ZaPR4b belongs to class II PR4 proteins. Subcellular localization results showed that ZaPR4 is mainly localized to plasma membrane. ZaPR4b is highly expressed in the leaves of Z. armatum. Treatment with SA significantly induced ZaPR4b expression and enhanced its resistance to leaf rust. The expression levels of ZaPR4b in the leaves of different varieties were positively correlated with leaf rust resistance, suggesting that ZaPR4b is involved in the defense response of Z. armatum to leaf rust.

