

Introduction
With the rapid development of the global economy and the increasing depletion of land resources, ocean development has become an important strategy for many countries [1]. Meanwhile, as an essential tourism resource, Sea island can greatly satisfy the people’s growing demand for leisure and entertainment [1, 2]. However, because the substrate of tropical coral islands is characterized by nutrient deficiency, high salinity, extremely low water content, and harsh climatic and environmental conditions such as high temperatures and strong light, it is difficult to form vegetation and the corresponding livable environment under natural circumstances [3-5]. It is necessary to prioritize plant species with high physiological and ecological adaptability to coral islands.
The tropical coral island group located in Sansha City, Hainan Province, China, is formed mainly by coral sand, bird droppings, and plant debris [6, 7] in a specialized ecological environment with extreme habitats such as seasonal drought, intense light, high temperature, high salt, tidal, typhoon, and nutrient-poor soil [6]. The soil is alkaline (pH between 7.72 and 8.63) and rich in elements such as calcium (Ca) and phosphorus (P) [2, 8]. Some of the islands’ natural vegetation has been degraded and urgently needs restoration due to extreme environments. Therefore, it is necessary to study plants’ physiological characteristics and to evaluate their adaptability to the harsh environment of tropical coral islands by determining plant functional traits.
Changes in plant functional traits reflect the plant’s adaptive strategies to environmental stresses and can be used to identify plant stress tolerance [9-11]. Under compound stress conditions such as drought, barrenness, high temperature, and intense light, plants usually exhibit higher starch and non-structural carbohydrate (NSC) contents to increase photosynthetic efficiency, reduce water transpiration, and mitigate intense light scorching [10, 11]. It has been suggested that the photosynthetic rate decreases before the respiration rate under prolonged drought stress, resulting in a decrease in NSC content, which can lead to plant death when non-structural carbohydrates fail to meet the metabolic demands of the cells [11-14]. In addition, in response to high temperatures and intense light damage in tropical coral islands, plant leaves usually exhibit lower chlorophyll content to minimize intense light damage [10-12].
The plant antioxidant enzyme system can reduce reactive oxygen species and minimize cellular damage when subjected to high temperatures and drought stress [9-12]. Specifically, superoxide dismutase (SOD) is a common antioxidant enzyme in leaf cells, and malondialdehyde (MDA) is one of the indicators for identifying plants damaged by adversity [12]. Besides, abiotic soil properties also affect plant performance. Soil water content is a direct source of plant water and directly affects physiological and ecological processes (e.g., transpiration and photosynthesis). Soil nutrients directly affect plant nutrient uptake [6, 10, 12].
To explore the differences in physiological adaptations of different plants introduced to the islands and to provide references for plant settlement, growth, and restoration in ecological planning and vegetation restoration [6, 9-16]. We selected three woody plants (Casuarina equisetifolia, Morinda citrifolia, and Scaevola taccada) growing in Guangzhou City and compared the leaf’s physiological and nutrient characteristics between Guangzhou City and coral island of Sansha City in China. This study hypothesizes that (1) the three plants’ physiological characteristics respond differently to the coral island; (2) adding garden soil to coral soil may improve the plant’s adaptations.
Materials and Methods
Study Area
The study area is located on coral island in Sansha City, Hainan Province, China (111°11′-112°54′E, 15°46′-17°08′N), with an average annual precipitation of 2000 mm, an average annual temperature of 32.3ºC [3, 8, 9]. The soil type of coral island is phosphatic limestone soil and alluvial coral sand, and soil mineral elements are mainly derived from coral gravel, seabird droppings, and plants [6, 9, 15]. Due to the soil’s high void space and poor water retention capacity, the plants would be susceptible to drought stress even if the coral island receives abundant rainfall throughout the year. The plant community of coral island occurs in mono-eugenic communities.
The nursery of the South China Botanical Garden of the Chinese Academy of Sciences is located in Guangzhou City, Guangdong Province, China (112°57’- 114°3’E, 22°26’-23°56’N), which has a subtropical monsoon climate, warm and humid, with plenty of heat and light, and a short frosty period in summer. The average temperature throughout the year is about 21.9ºC. The average relative humidity is 77%, and the annual rainfall is about 1,900 mm. The soil type of the garden is laterite.
Plot Setting and Sample Collection
We selected two sampling sites on coral island in October 2023, labeled S1 and S2. In contrast to the S2 sampling site, the S1 sampling site consisted of a uniform spread of garden soil (laterite) on the surface of the original coral soil. Then, we selected the single community of C. equisetifolia, M. citrifolia, and S. taccada within the S1 and S2 sampling sites and randomly set up three 5 m × 5 m sample plots within each single community. We collected their mature leaves in plastic bags. Meanwhile, the single community of C. equisetifolia, M. citrifolia, and S. taccada (planted at the same time as coral island) were selected from the nursery of the South China Botanical Garden of the Chinese Academy of Sciences in Guangdong Province, China (labeled as CK). Three 5 m × 5 m sample plots were randomly set up within each single community, and we also collected the mature plant leaves in plastic bags.
Leaf Samples Chemical Analyses
The leaves were oven-dried at 105ºC for 30 minutes and then dried at 65º for at least 72 hours until a constant weight. Dried leaves were ground to powder and passed through a 0.25 mm (60 mesh) sieve. The leaf carbon (C), nitrogen (N), P, potassium (K), and δ13C contents were measured by using an elemental analyzer. The Ca content was measured using a photometer after digesting the samples in H2SO4-H2O2 [17-18]. Leaf water content (LWC) was measured by the drying-weighing method. Finally, we calculated the C:N, C:P, and N:P according to the following equations:
The thiobarbituric acid method determined the leaf’s MDA content [19]. The SOD activity was determined by xanthine oxidase method [20]. The soluble protein content was determined by Coomassie bright blue staining, and the reduced glutathione (GSH) content was determined by the method mentioned by Liu [12].
Leaf Non-Structural Carbohydrate Analyses
The dried leaf samples were pulverized in a ball mill, and the soluble sugar and starch contents were determined by the Anthrone colorimetric method, which was determined and calculated using the maximum absorption value at 620 nm by spectrophotometer (UA1880, Jinghua Instruments, China).
Determination of Photosynthetic Pigments
The fresh leaves (500 mg) from three trees per species were split into three groups and homogenized with 10 mL acetone (80%), and then chlorophyll was extracted from the homogenized plant materials to avoid light for 1-2 days. The absorbance of the supernatant was read at 645 nm, 663 nm, and 470 nm using a spectrophotometer (UA1880, Jinghua Instruments, China). The total chlorophyll content was calculated according to the following equation:
Fig. 1.
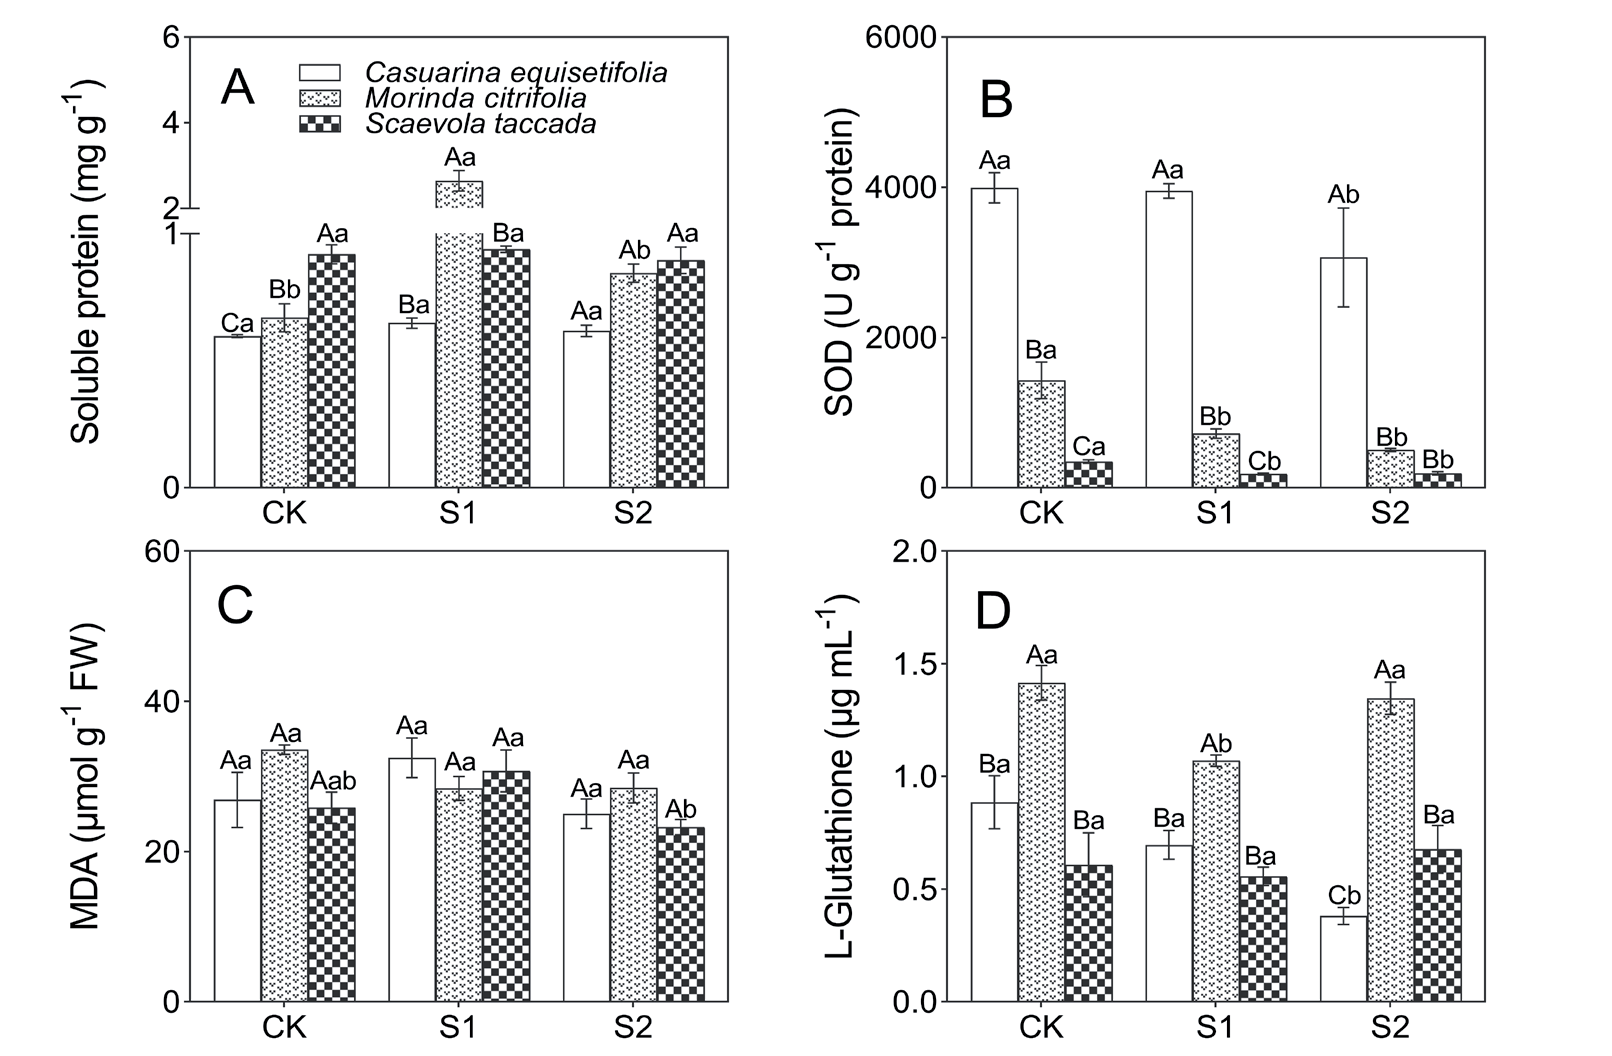
Soluble protein (A), superoxide dismutase (SOD, B), malondialdehyde (MDA, C), and L-Glutathione (D) of three plants (Casuarina equisetifolia, Morinda citrifolia, and Scaevola taccada) at three sites (CK, S1, and S2). Values are mean ± standard error (n = 3). Uppercase letters show significant differences between the three plants (p<0.05). Lowercase letters show significant differences between the means of CK, S1, and S2 (p<0.05).
Plants’ Adaptability Evaluation
To evaluate the adaptation of the three plants in the island, the data set method was employed to establish a dimensionless score (si) between 0 and 1 using the following equation: si = (xi – xmin)/(xmax – xmin), where si is the score of the ith indicator, xi, xmax, and xmin are the measured, maximum, and minimum values of the ith indicator, respectively.
Statistical Analysis
One-way analysis of variance (ANOVA) was used to examine differences between sample plots and plant species in leaf properties. Data were processed and analyzed using Excel 2020 and SPSS 22.0 software and further graphed using GraphPad Prism 8 software. Pearson’s correlation analysis and Mantel’s test were performed using R studio 4.1.1 (hmisc, corrplot, vegan, dplyr, ggcor, and ggplot2 packages).
Fig. 2.
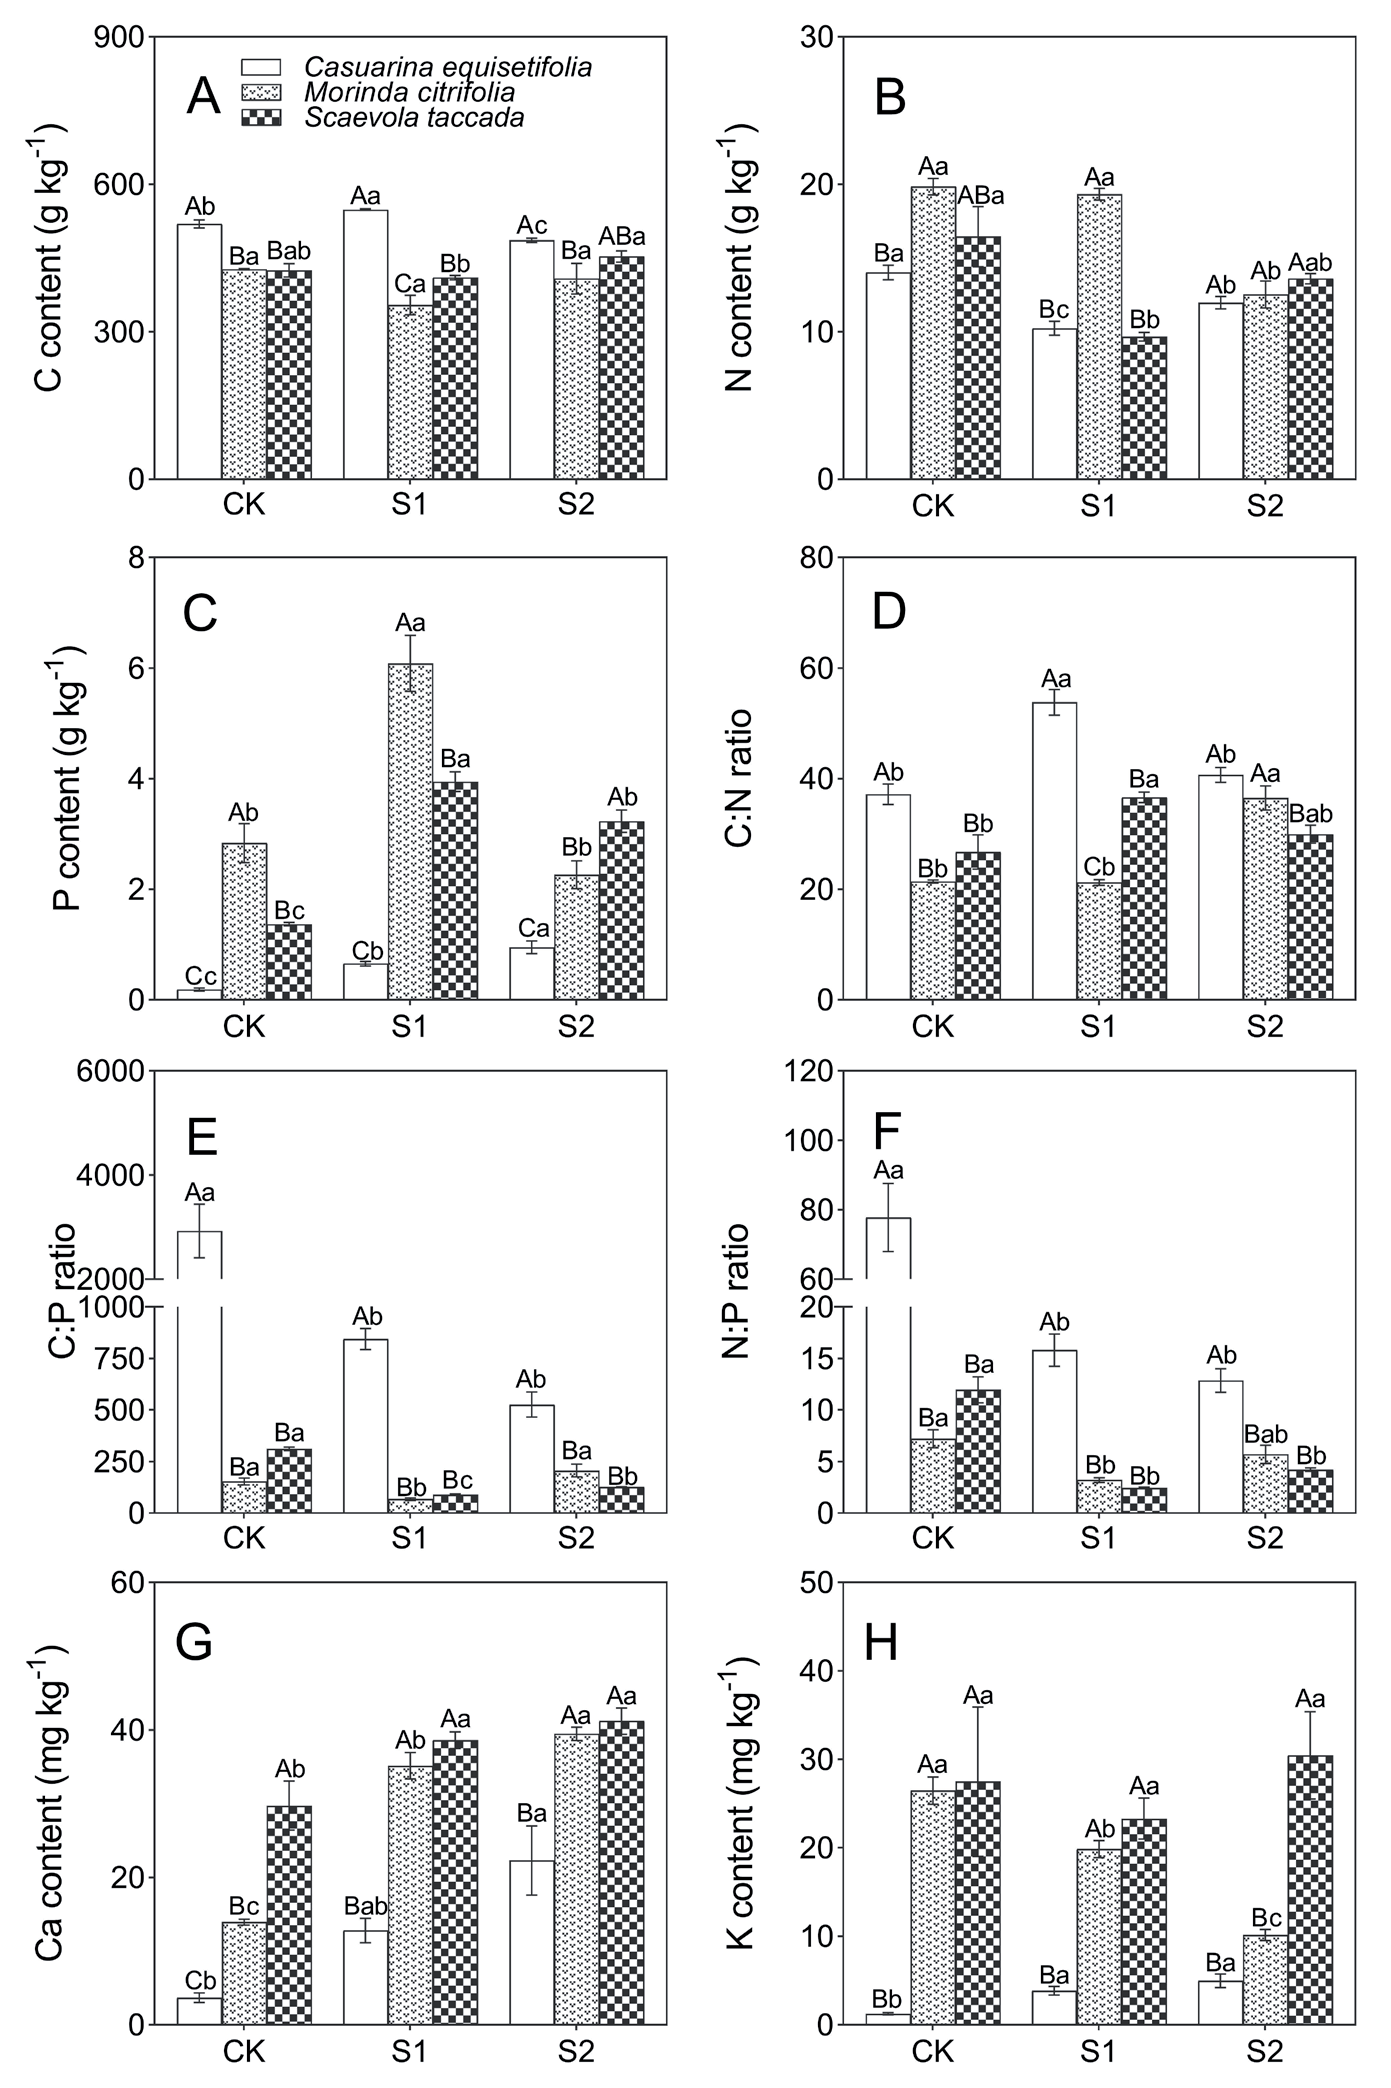
Leaf C (A), N (B), P (C), C:N ratio (D), C:P ratio (E), N:P ratio (F), Ca (G), and K content (H) of three plants (Casuarina equisetifolia, Morinda citrifolia, and Scaevola taccada) at three sites (CK, S1, and S2). C, carbon; N, nitrogen; P, phosphorus. Values are mean ± standard error (n = 3). Uppercase letters show significant differences between the three plants (p<0.05). Lowercase letters show significant differences between the means of CK, S1, and S2 sites (p<0.05).
Results
Leaf Physiological Properties
The leaf SOD activity of M. citrifolia grown at the S2 site on the tropical coral island was significantly lower by 64.84% than M. citrifolia grown in Guangzhou (p<0.05, Fig. 1). Additionally, at three sites, the SOD activity of C. equisetifolia was higher than M. citrifolia and S. taccada; the L-Glutathione content of M. citrifolia was higher than C. equisetifolia and S. taccada.
Leaf Nutrient Absorption, C, N, P Stoichiometry, And K, Ca Element
Compared with C. equisetifolia and S. taccada grown in Guangzhou, those grown at the S1 and S2 sites on coral island had significantly higher leaf P contents and lower leaf N:P ratios (p<0.05, Fig. 2). Besides, at all three sites, C. equisetifolia had lower leaf P content, higher leaf C:N ratios, higher C:P ratios, and higher N:P ratios than M. citrifolia and S. taccada (p<0.05). There was a significant difference in the leaf K content in M. citrifolia between the CK and S2 sites (p<0.05).
Leaf Photosynthetic Pigments
Leaf carotenoid content, chlorophyll-a content, chlorophyll-b content, and total chlorophyll content were lower in the three plants (C. equisetifolia, M. citrifolia, and S. taccada) grown at the S1 and S2 sites on coral island compared to the three plants grown in Guangzhou (Fig. 3).
Leaf Water Content, δ13C, NSCs, and Soluble Sugar: Starch
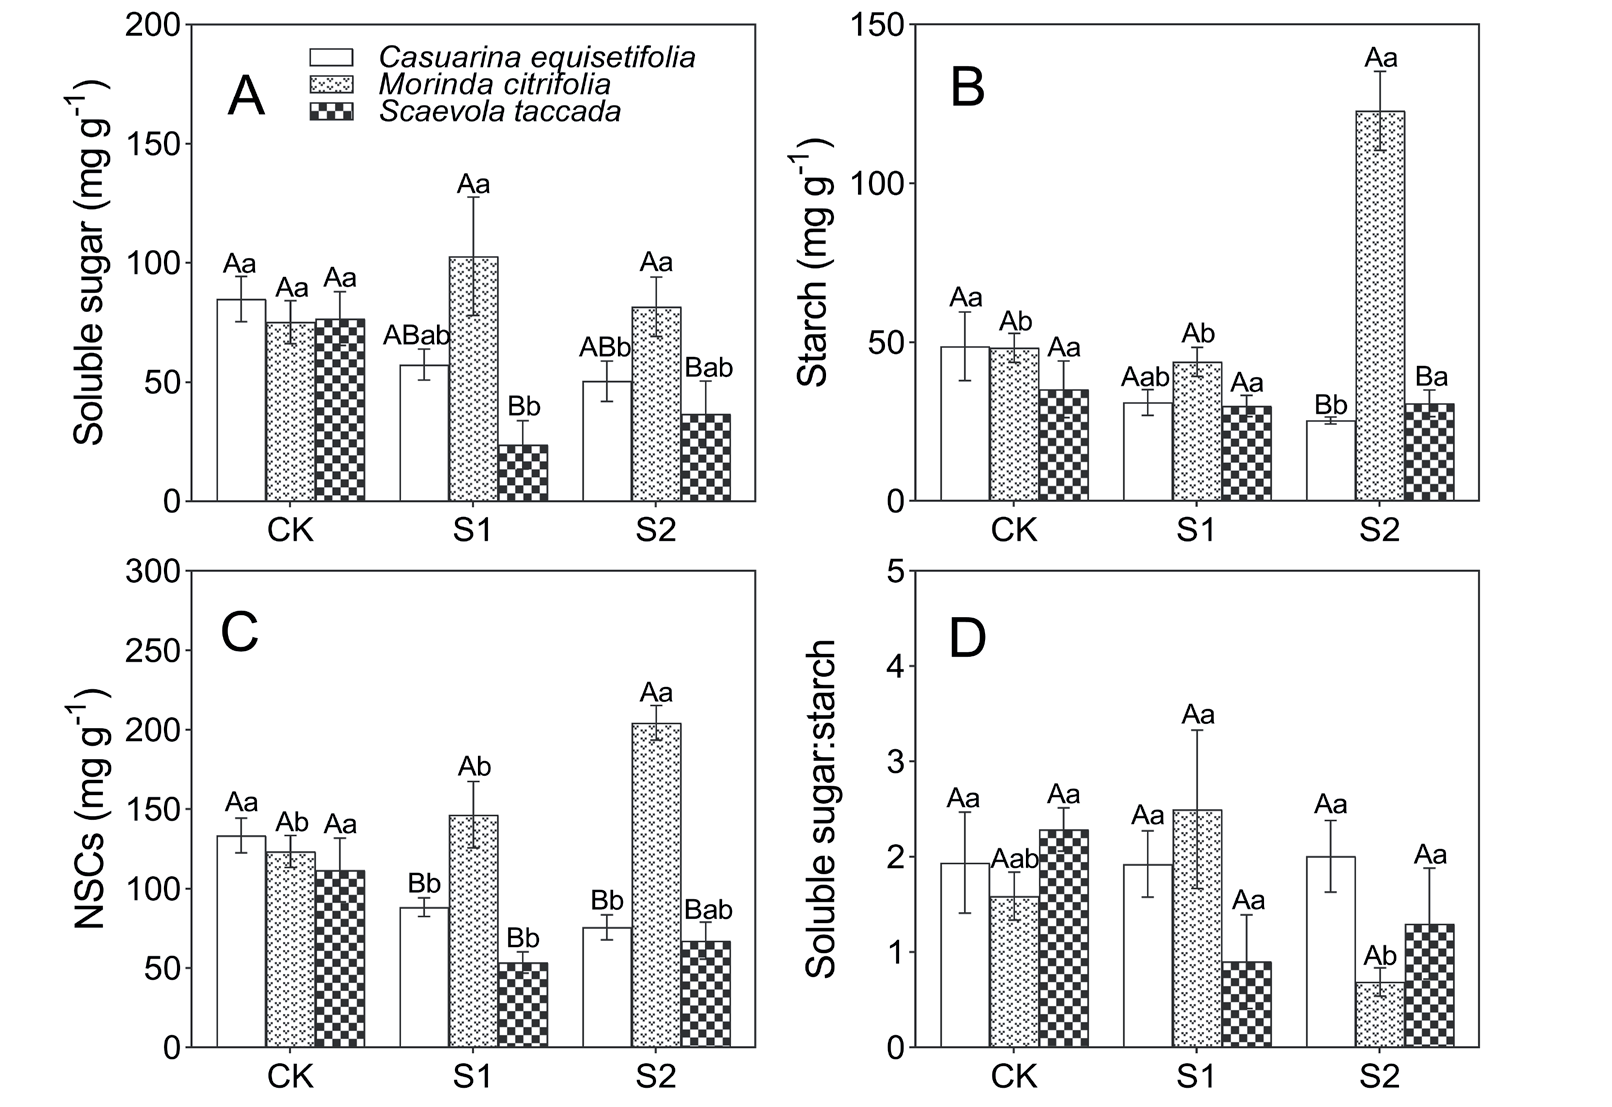
There were no significant differences in the leaf water content of the three plants at the three sites (CK, S1, and S2). Besides, among the three plants, S. taccada had the highest leaf water content (Fig. 4). Leaf δ13C content was significantly lower in the three plants (C. equisetifolia, M. citrifolia, and S. taccada) grown at the S1 and S2 sites on coral island compared to the three plants grown in Guangzhou (p<0.05). Besides, the leaf’s soluble sugar and NSC content of S. taccada grown at the S1 and S2 sites on coral island were significantly reduced by 69.07% and 52.35%, 52.01% and 39.80% than grown in Guangzhou (p<0.05, Fig. 5).
Ranking of Three Plants’ Adaptability to Coral Island
The comprehensive subordinate function mean values showed the highest value in M. citrifolia (0.44), followed by S. taccada (0.31) and C. equisetifolia (0.29), which indicated that M. citrifolia had the best adaptability to the extreme environment of the coral island among the three plants.
Fig. 3.
Carotenoid content (A), chlorophyll-a content (B), chlorophyll-b content (C), and total chlorophyll content (D) of three plants (Casuarina equisetifolia, Morinda citrifolia, and Scaevola taccada) at three sites (CK, S1, and S2). Values are mean ± standard error (n = 3). Uppercase letters show significant differences between the three plants (p<0.05). Lowercase letters show significant differences between the means of CK, S1, and S2 sites (p<0.05).
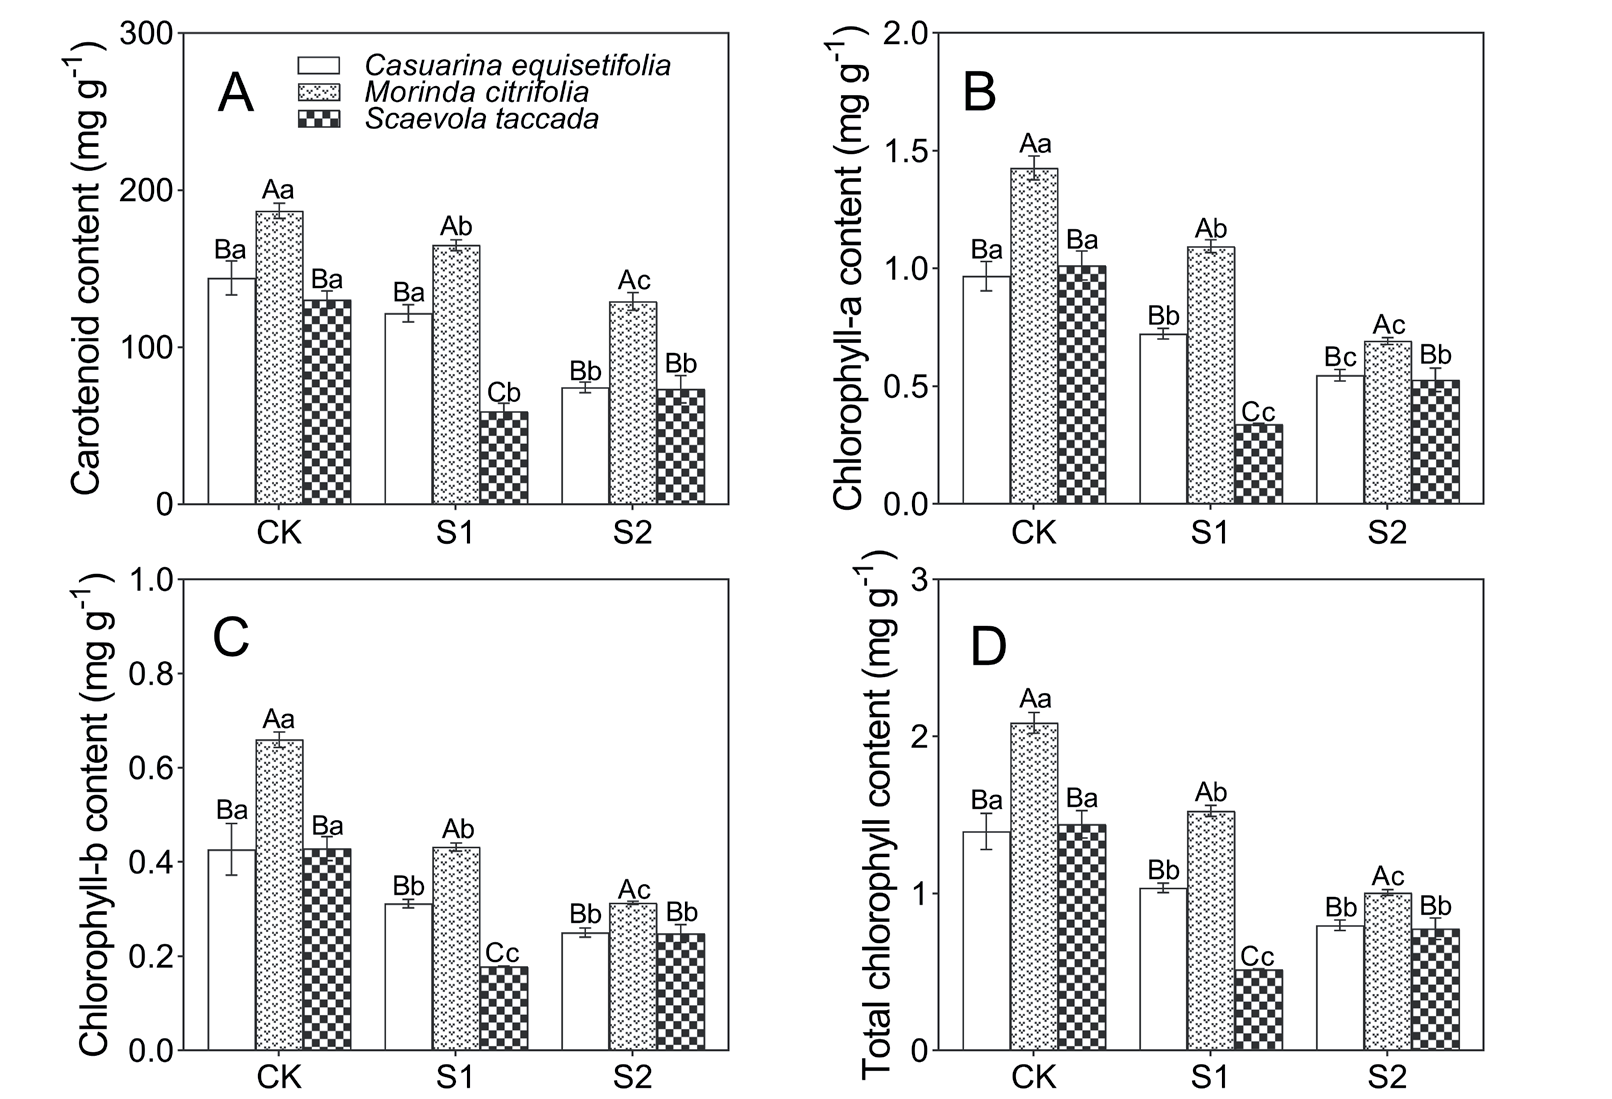
Fig. 4.
Leaf water content (A) and δ13C content (B) of three plants (Casuarina equisetifolia, Morinda citrifolia, and Scaevola taccada) at three sites (CK, S1, and S2). Values are mean ± standard error (n = 3). Uppercase letters show significant differences between the three plants (p<0.05). Lowercase letters show significant differences between the means of CK, S1, and S2 sites (p<0.05).
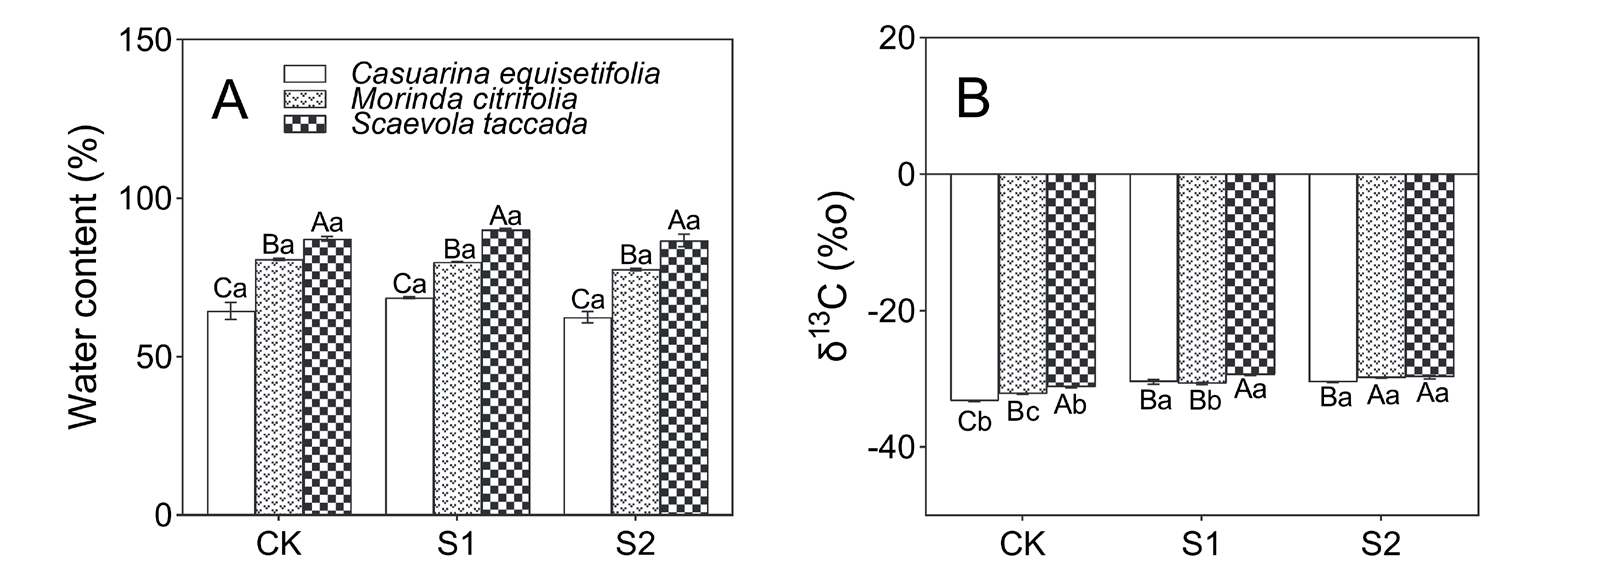
Fig. 5.
Leaf soluble sugar (A), starch (B), NSCs (C), and soluble sugar:starch ratio (D) of three plants (Casuarina equisetifolia, Morinda citrifolia, and Scaevola taccada) at three sites (CK, S1, and S2). Values are mean±standard error (n = 3). Uppercase letters show significant differences between the three plants (p<0.05). Lowercase letters show significant differences between the means of CK, S1, and S2 sites (p<0.05).
Correlation of Leaf Characteristics with Soil Properties
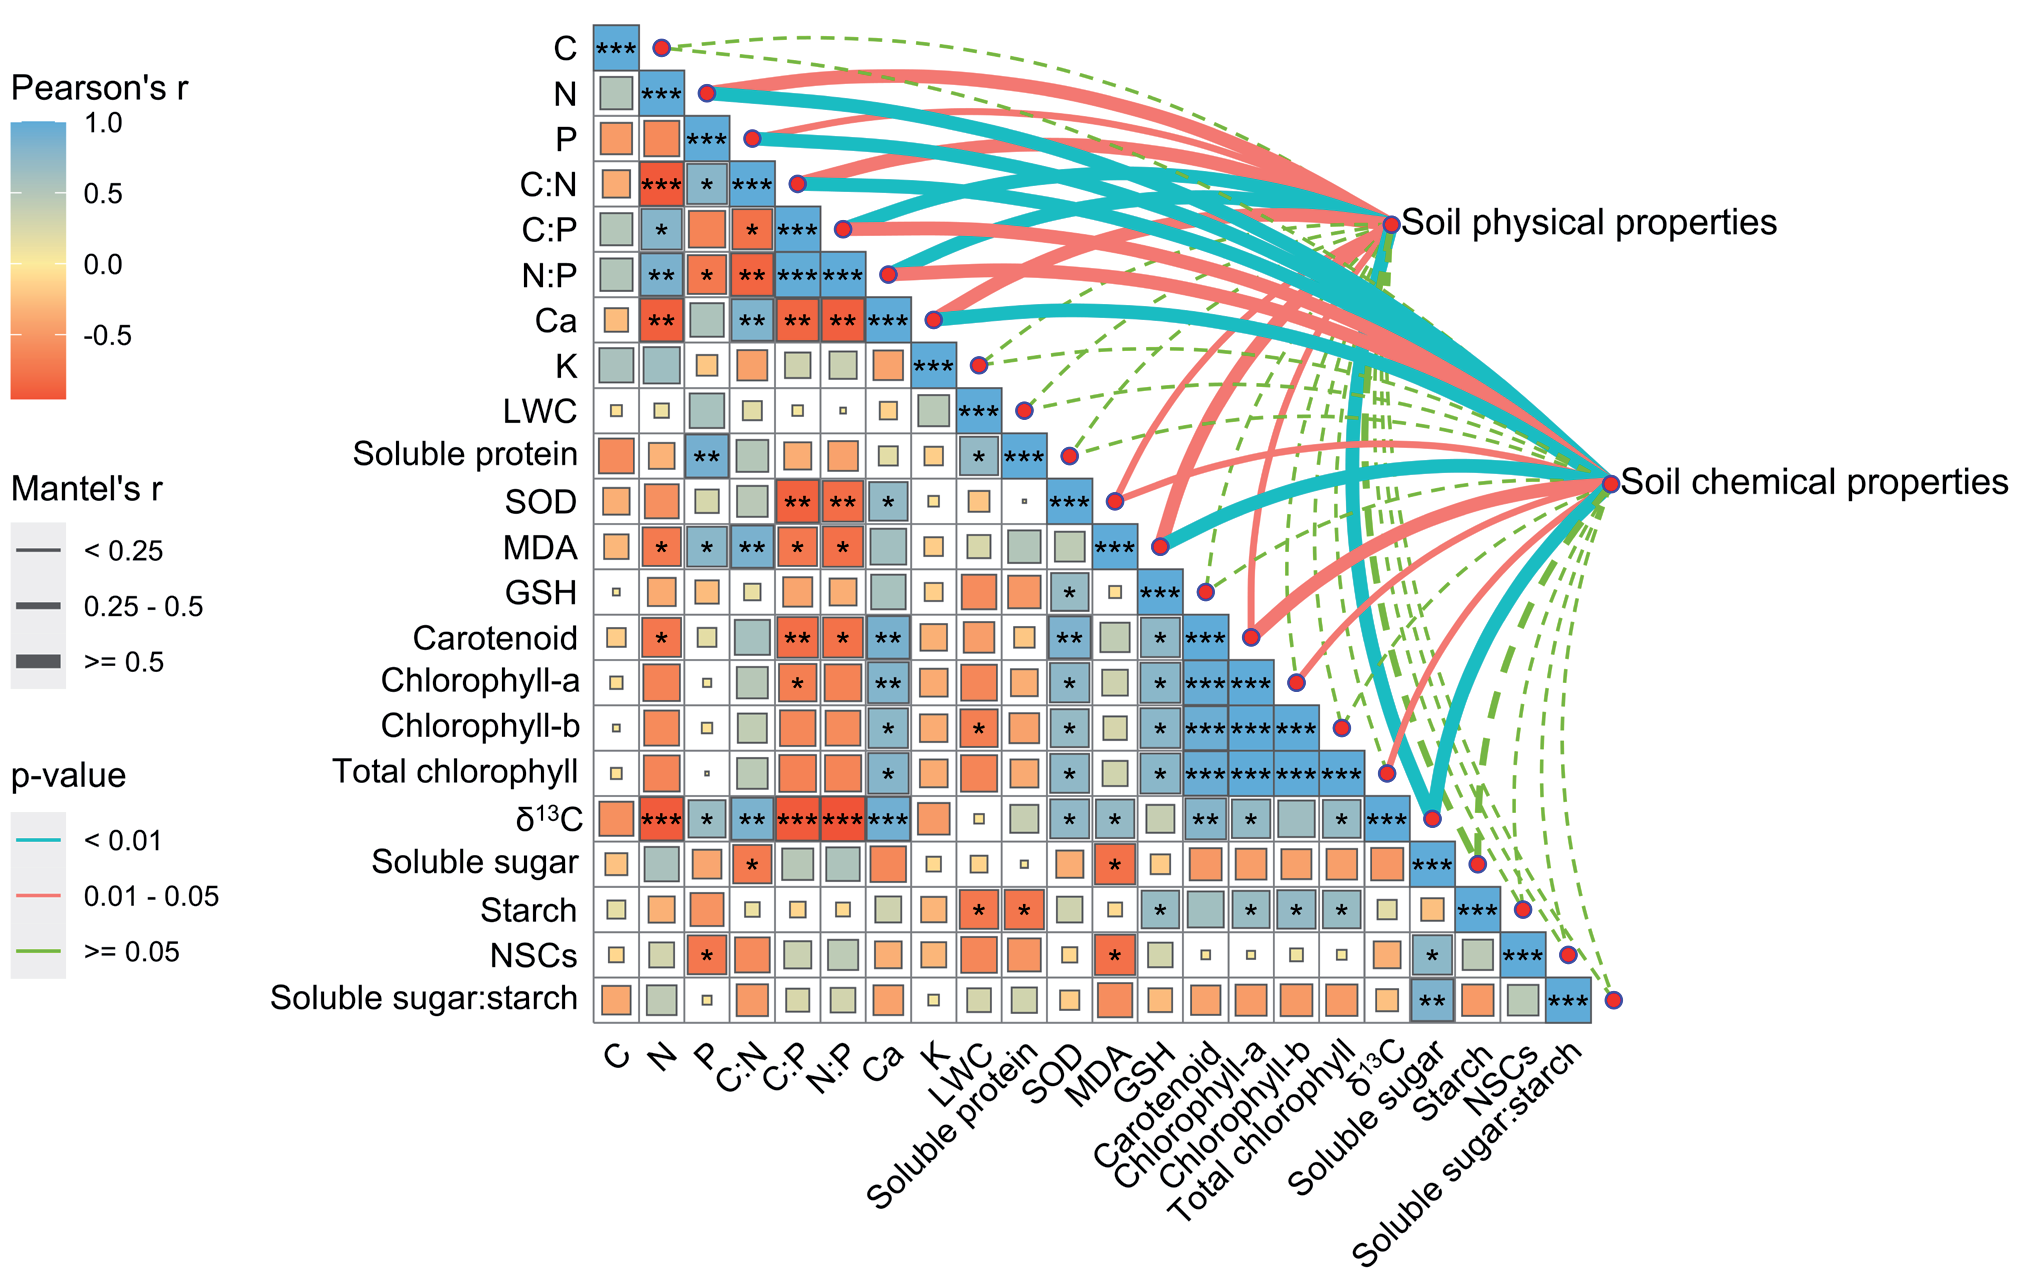
Noteworthy observations were made regarding the significant and positive correlations observed between leaf photosynthetic pigments with leaf Ca content, SOD activity, and L-Glutathione content of three plants on a tropical coral island (p<0.05, Fig. 6). Through Mantel test analysis, it was established that soil physical properties (pH, BD, and water content) were notably linked with leaf N, P, C:N ratio, C:P ratio, N:P ratio, Ca, SOD activity, MDA activity, carotenoid, and δ13C indicators (p<0.05). This significant correlation was also evident in soil chemical properties (SOC, total N, total P, NO3--N, NH4+-N, and available P) with leaf N, P, C:N ratio, C:P ratio, N:P ratio, Ca, SOD activity, MDA activity, carotenoid, total chlorophyll, and δ13C contents (p<0.05).
Discussion
Tropical coral islands are ecologically harsh (seasonal drought, high salinity, strong alkalinity, high temperature, and strong light), and plant leaves are most susceptible to stress. 90% of the plant’s biological three sites (CK, S1, and S2). *, **, and *** indicate that the significance level at p<0.05, p<0.01, and p<0.001, respectively. production is leaf photosynthesis [10, 17, 21-23]. Therefore, more attention needs to be paid to plant leaves’ response to the harsh environment of tropical coral islands.
Fig. 6.
Correlation analysis of leaf water content (LWC), element characteristics (Ca and K), nutrient absorption (C, N, P, C:N ratio, C:P ratio, and N:P ratio), non-structural carbohydrate (NSCs, soluble sugar, starch, and soluble sugar:starch ratio), leaf δ13C content, leaf physiological properties (soluble-protein, SOD, MDA, and GSH) and photosynthetic pigment contents (carotenoid, chlorophyll-a, chlorophyll-b, and total chlorophyll) with soil physical (pH, BD, and soil water content) and chemical properties (soil organic carbon, total N, total P, NO3 --N, NH4 +-N, and available P) of three plants (Casuarina equisetifolia, Morinda citrifolia, and Scaevola taccada) at three sites (CK, S1, and S2). *, **, and *** indicate that the significance level at p<0.05, p<0.01, and p<0.001, respectively.
This study supported the first hypothesis that the three plant’s leaf physiological properties respond differently to the coral island. SOD activity indirectly reflects the antioxidant capacity of plant tissues [24- 28]. Compared with C. equisetifolia and M. citrifolia grown in Guangzhou, those grown at the S2 site on coral island had lower leaf SOD activity, which may be attributed to the inherent growing environment of coral islands, then leads to oxidative stress in the plant, thus resulting in decreased leaf SOD activity. Quantifying chlorophyll content is a pivotal metric in evaluating the plant’s photosynthetic capacity, given its crucial role in accelerating photosynthesis and subsequent organic matter accumulation [12, 28]. Chlorophyll-a is primarily a photosynthetic light reaction center pigment, and the decrease in chlorophyll-a contributes to reducing the excess light energy transfer to the reaction centers of the plant photosynthetic system, which can reduce damage from bright light [3, 12]. Compared to plants grown in Guangzhou, plants grown in tropical coral islands have lower chlorophyll content, which may be because when the light intensity is too high, the phenomenon of photoinhibition may be generated for plants; therefore, lowering the chlorophyll content is an important way for plants to avoid capturing overload energy leading to photoinhibition [12, 17].
The potential effects of the coral island environment on plant growth have been explored in various studies [9, 14]. This investigation focuses on elucidating the impact of the coral island environment on plant nutrient content, with particular attention to C, N, and P stoichiometry. The content and stoichiometric ratios of C, N, and P hold pivotal significance in maintaining optimal plant health and growth dynamics [27]. The C:N ratio reflects the plant’s capacity to assimilate C via nutrient uptake, characterizing C and N metabolism coordination [27, 28]. Similarly, C: P and N: P ratios play vital roles in gauging growth rates and the potential nutrient limitations experienced by plants [27, 28]. Leaf N: P ratio was lower in the three plants (C. equisetifolia, M. citrifolia, and S. taccada) grown at the S1 and S2 sites on coral island compared to those in Guangzhou. Significantly, the N: P ratio in leaves correlates with plant growth rates and N and P uptake efficiency [9, 27]. This study corroborates these findings, highlighting that introducing the plant to P-rich islands may boost plant P uptake and induce shifts in C:N, C:P, and N:P ratios, with plant growth being more N-limited. Notably, the leaf Ca content of the three plants grown at the S2 site on coral island was markedly elevated compared to that grown in Guangzhou. This observation underscores the superior ability of the coral island to enhance leaf Ca assimilation, likely due to the specific coral island environments.
Sugars in leaf NSCs are the main energy source of plants, and as important substances involved in the plants’ life process, they largely determine the plants’ adaptability to the environment [9]. When plants suffer from drought stress, they will reduce water loss by closing their stomata, which in turn leads to a decrease in their photosynthetic rate. When the photosynthetic rate is reduced to the point that newly synthesized carbohydrates are insufficient to satisfy the plant’s growth and metabolism, they will consume the plant’s own stored NSCs [10-13, 28, 29]. In this study, the soluble sugars and NSC contents of C. equisetifolia and S. taccada grown on the S1 and S2 sites of the tropical coral island were lower than those grown in Guangzhou, whereas soluble sugars and NSC contents of M. citrifolia showed the opposite trend, suggesting that M. citrifolia is better adapted to the harsh environment of the tropical coral island than C. equisetifolia and S. taccada.
Soil characteristics are important environmental factors influencing plant growth [24-27]. In this study, both S1 and S2 sampling sites were located in the same small area with the same climatic environment on coral island, Sansha City, Hainan Province, China. Compared with C. equisetifolia and M. citrifolia grown in the S2 site, those grown at the S1 site on coral island had higher leaf SOD activity. Notably, the observed lower photosynthetic pigment contents of C. equisetifolia and M. citrifolia in the S2 sampling site compared to the S1 sampling site may stem from plants’ direct assimilation of soil-available nutrients under conditions of garden soil incorporation, potentially increasing chlorophyll synthesis [3, 9, 17]. Similar to the findings of previous studies [29-32], we also found that soil composition plays an important role in plant responses to harsh environments (Fig. 6). In this study, garden soil contains more nutrients than coral soil, and amending coral soils by adding garden soil may help improve plant physiological adaptations.
Conclusions
Coral islands’ stressful environments (high temperature, drought, intense light, and salinity) have important impacts on plant survival and growth. Therefore, plants and their ability to adapt to harsh environments should be considered when selecting potentially suitable plants for island revegetation. This study showed that among the three plants (C. equisetifolia, M. citrifolia, and S. taccada), M. citrifolia showed the best physiological adaptation. M. citrifolia adapts to coral island environments through reduced SOD activity, elevated soluble protein content, and reduced photosynthetic pigments to increase tolerance to environmental stress. This study provides basic data on the physiological responses and nutrient absorption of three woody plants grown on coral islands, an important reference value for revegetation and restoration of tropical coral islands. However, due to the complexity of the relationship between the environment and species, the mechanism of climate, soil, and microbial factors that affect plants’ physiological and ecological adaptations needs further investigation.

