

Introduction
Organs in plants, such as leaves, stems, roots, and flowers, contain many active chemical substances. These substances include various intermediary products of metabolism known as metabolites, and all plants produce between 100,000 and 1 million metabolites overall [1]. Based on their assumed functions, metabolites are grouped into primary and secondary metabolites [2]. As primary metabolites are associated with vital plant physiological processes, they are present in every plant species and play a direct role in development, growth, and reproduction. [3, 4]. On the other hand, secondary metabolites do not directly contribute to the growth, development, or reproduction of plants; instead, they perform highly specific activities under very specific conditions. Their activities include enhancing plant growth, adjusting to shifting environmental circumstances, fortifying plants’ resistance to abiotic stresses, and shielding plants from environmental harm and pathogen infection. [4, 5].
Although A. Kossel coined the word "secondary" in 1891, the term implies that secondary metabolites are present only incidentally and are not important for plant life, whereas primary metabolites are found in every live cell that can divide [6]. It is commonly accepted that plant defense mechanisms against biotic stressors are involved in the biosynthesis of several secondary metabolites [7]. Ncube and coworkers [8] reported that plants produce a vast array of secondary metabolites in response to various biotic stressors, and the chemical makeup of each metabolite is complicated. Plant defense systems become activated when a signal from outside or inside the cell reaches the system through a receptor on the plasma membrane. The binding of a receptor to a signal molecule initiates a signal transmission cascade that results in the stimulation or manufacture of transcription factors, which modulate the function of biosynthetic genes in plants that regulate secondary metabolism [9].
Based on their methods of synthesis, secondary metabolites are typically divided into the following major categories: alkaloids, terpenes, and phenolics [10, 11]. These phytochemicals are species- and organ-specific and show remarkable chemical and biological diversity [12].
Secondary metabolites from plants are utilized as food additives, agrochemicals, tastes, perfumes, colors, and biopesticides [13]. Currently, many of these compounds are extracted from naturally grown entire plants via solvent extraction; consequently, many valuable and even endemic species have become extinct due to the ongoing destruction of plants, which has posed a serious threat to plant species recovering access to their native habitats [14, 15]. Furthermore, a wide range of environmental conditions, such as temperature, light, soil fertility, soil water, and salt, control secondary metabolite accumulation in plants. The concentration of secondary metabolites in most plants can be altered when one of these parameters changes, even when other factors remain constant [16]. As a result, secondary metabolites are naturally produced in low quantities in plants, and large quantities of plant material are needed to extract meaningful quantities of these molecules. The isolation of these substances was limited to wild plant-based substances, resulting in overharvesting and loss of significant plant species [17]. Other challenges involved in the extraction of metabolites from intact plants include geopolitical and environmental instabilities, limited knowledge of metabolite biosynthesis and signal transduction pathways, slow growth of certain plants, low yields in nature, and unexpected variability in accumulation [18]. Furthermore, large-scale production of the source plant may be unfeasible in some cases due to environmental, ecological, or climatic considerations, as well as a shortage of agricultural land [19].
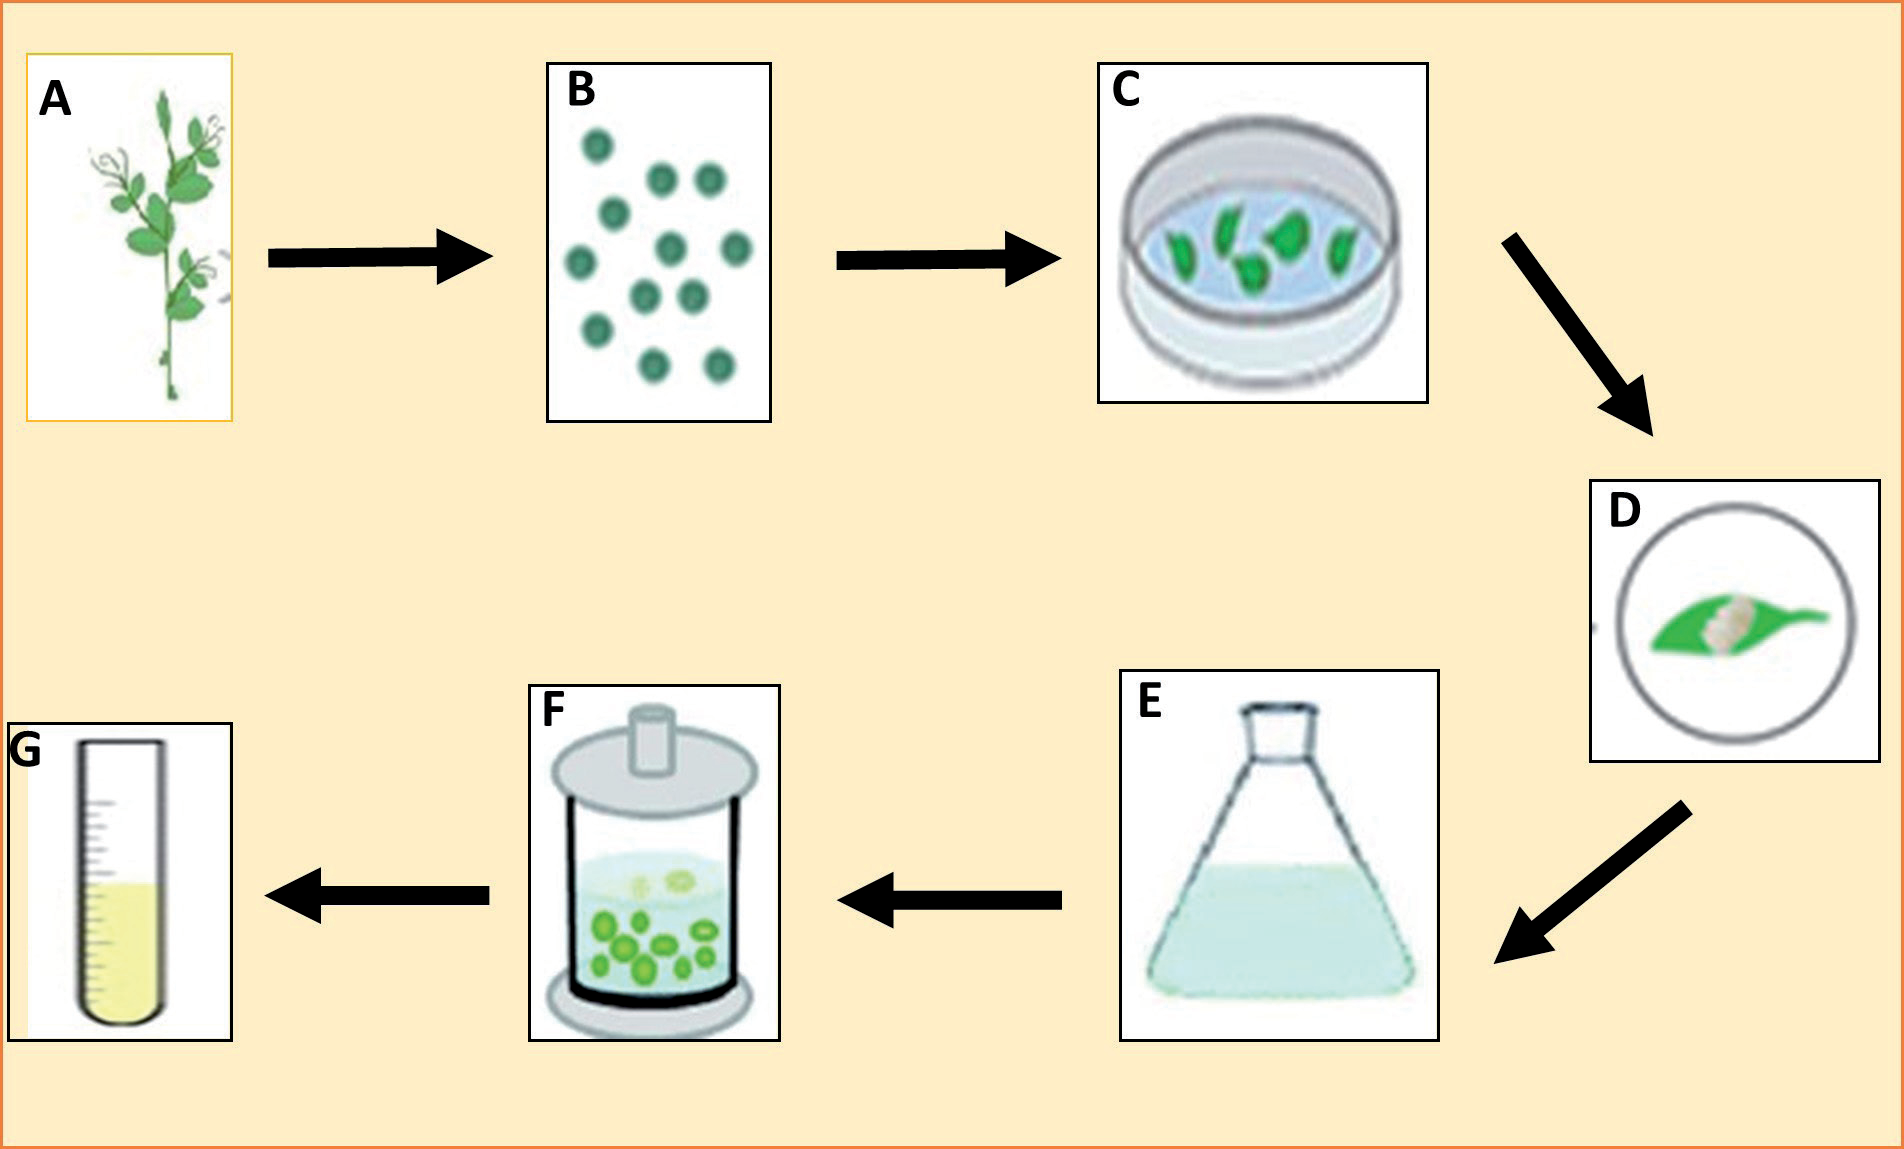
An alluring alternative to conventional cultivation methods for gathering plants from the wild to produce high-value secondary metabolites is plant cell suspension culture. To establish cell suspension cultures, friable calluses are often inoculated into a liquid medium in flasks and then placed on a rotating shaker. A cell suspension culture is created as the newly generated cells spread across the liquid medium. The suspended cells are moved to new media after two to three weeks, and the larger pieces are thrown away (Fig. 1). Compared to cells in callus culture, cells in suspension can exhibit substantially greater rates of cell division. Thus, when rapid and large-scale cell production is needed, cell suspension works best [20-23].
Fig. 1.
Plant cell suspension cultures induction and secondary metabolite production. (A) Main plant and explant sources, (B) Isolation of explant, (C) Sterile explant on callus induction medium (D) In vitro callus induction (E) Cell suspension culture (F) Bioreactor (G) Isolation of secondary metabolites.
Instead of using intact plants, suspension cultures can produce useful compounds under controlled conditions that are unaffected by soil or climate changes. Cultured cells easily reproduce to generate the specific metabolites of any plant cell, and automated controls may be applied to produce secondary metabolites and regulate cell proliferation [24].
Plant cell cultures preserve the wild populations of species and are inexpensive to create and maintain. Additionally, many posttranslational modifications that occur in plant cells seldom occur in prokaryotes, and overexpressing heterologous genes is much easier now due to the discovery of novel gene-editing techniques [25]. Moreover, establishing synthetic biotechnology methods for plants and creating biofactories using plant cells for the synthesis of secondary metabolites is impossible [26-28].
A multitude of recent reviews, including those by Chandran et al. [23], Rahmat and Kang [29], Cardoso et al. [30], Gutierrez-Valdes et al. [31], Marchev et al. [32], and others, discuss the use of plant tissue culture for the synthesis of secondary chemicals. In this review, we focused on the status, limitations, and methods for overcoming these circumstances when employing plant cell suspension culture as a potential tool for plant secondary metabolite production. We also suggest biotechnological strategies that may be helpful in boosting the production of secondary metabolites in in vitro produced plant cell suspension cultures.
Historical Background
For a long time, it has been known that plant cell culture can generate a wide range of secondary metabolites [33]. In 1956, Routien and Nickell, working with the American pharmaceutical company Pfizer Inc., submitted the first patent for mass cell culture of plant tissue and metabolite synthesis [34]. In the late 1960s, researchers determined that plant cell cultures could be used to produce important chemicals, particularly chemicals for the development of new drugs. Diosgenin was successfully isolated from Dioscorea deltoidea suspension cells by Kaul and Staba [35]. The suspension cells that were 3–4 weeks old had the highest diosgenin concentration (1.02%), while the differentiated cells only displayed negligible levels of diosgenin. In a different investigation, Heble et al. [36] effectively isolated diosgenin from Solanum xanthocarpum, demonstrating that diosgenin develops in large amounts in tissue culture.
At an international convention held in Munich in 1976, researchers revealed the remarkable metabolic capacities of plant cells and the unexpected diversity of plant cell biosynthetic capacity, which may explain the earlier inconsistency in the results. This natural diversity is used to find cultures with high yields for industrial applications [37-40]. Since the late 1970s, the number of patent applications filed in this domain has significantly grown, particularly in the science and business sectors in Japan and Germany. In 1983, for the first time, Mitsui Petrochemical Industries Ltd. of Japan succeeded in producing a dye known as shikonin from cell culture that exhibits anti-inflammatory and antibacterial characteristics [41]. Although shikonin production is a major accomplishment, researchers have discovered that a large proportion of cultivated plants cannot produce compounds that are characteristic of their ancestors. Morphine, tropane, and quinolone alkaloids, for example, are produced in very low quantities in cell cultures [42]. As a result, following a rise in interest, the research pattern decreased in the late 1980s and early 1990s, mainly because of poor rates of plant cell culture growth and the high capital expenses involved.
Status and Constraints
To survive, adapt to their surroundings, and protect themselves, plants synthesize a large variety of specialized secondary metabolites (over 200,000) [43]. Additionally, research efforts on utilizing plant secondary metabolites as potential natural alternative drugs for humans or livestock have gained momentum due to the detrimental impacts of utilizing antibiotics and other synthetic substances on human and animal health, as well as their safety and product quality [44]. Recently, the use of plant cell suspension culture to produce high-value plant-derived secondary metabolites of commercial interest has gained increasing attention [17, 45]. Based on recent advancements in molecular biology, plant cell culture, fermentation technology, and enzymology, these systems will become potential sources of key secondary metabolites [46]. Compared to tissue and organ culture, plant cell culture is a faster and more efficient approach to producing large amounts of secondary metabolites for industrial use. This approach is the most reliable and dependable method for producing natural products [47] and has been proposed to be extremely feasible [27]; this method is not constrained by the seasons [48], is more reliable than gathering plants from the wild [22], and offers a cost-effective alternative to conventional growing methods for producing metabolites and proteins [26, 28]. Moreover, the application of a bioreactor system for extensive plant cell culture to produce important bioactive chemicals is a current area of interest [49]. Thus, research on the production of secondary metabolites from cultivated plant cells has become a focus of researchers in a variety of biotechnological programs.
The synthesis of secondary metabolites in plant suspension cultures was recorded for a variety of plants (Table 1). Recent research has shown that secondary metabolites can be produced in vitro using plant cell cultures [23, 29-32]. Plant cell suspension cultures have been utilized to cultivate products such as shikonin, taliglucerase alfa, and Taxol in bioreactors [50]. An excellent model for industrial use was obtained in a recent attempt to synthesize paclitaxel utilizing plant cell cultures rather than extraction from complete plants [51]. In recent years, cell suspension cultures have been used to produce secondary metabolites at a pace comparable to or better than that of entire plants [52]; however, the technology still faces a variety of constraints in producing these metabolites. Product yield variability across several passages has prevented this technology from being applied in a successful and long-lasting manner [53]. The limitations to this method include poor cell efficiency, delayed development, genetic instability in high-producing cell lines, poor regulation of cellular division, high costs, the inability to maintain photoautotrophic growth, and contamination that results in significant losses in large-scale liquid cultures [33]. Moreover, Wilson and Roberts [21] reported that the generation of metabolites might be greatly influenced by gene silencing in a secondary metabolic pathway. Additionally, much of the research on this topic has been conducted by researchers affiliated with the business sector, is unpublished, and is not accessible to academic institutions. Moreover, plant cell suspension cultures have been shown to be extremely susceptible to environmental conditions, such as heat and medium components [54]. Verma and Shukla [55] reported that the production instability likely results from genetic, ecological, or epigenetic factors, resulting in inhomogeneity among cultures characterized by diverse groups. According to Hall and Yeoman [56], a secondary metabolite was created by a small portion of cells in the medium, and boosting yield frequently increased the percentage of competitive cells. Alterations in inter-and intracellular interactions are another possibility because the change in trend between gains and falls in the rate of production is not monotone [57]. This process seems to be organized and not autonomous of other cells, implying that cells can produce chemical signals for secondary metabolite formation during the culture cycle.
Table 1.
Bioactive secondary metabolites from plant suspension cultures of representative plant species.
[i] Abbreviations: MS: Murashige and Skoog medium, LS: Linsmaier and Skoog medium, BAP: 6-benzyl amino purine, NAA: α-naphthalene acetic acid, 2,4-D: 2,4-Dichlorophenoxyacetic acid, KN: Kinetin, IBA: indole-3-butanoic acid, 2-iP: N6 -(2-isopentenyl) adenine, TDZ: 1-phenyl3-(1,2,3-thiadiazol-5-yl)-urea, GA3: Gibberellic acid.
A typical difficulty in developing a large-scale cell culture production system is the progressive decrease in secondary metabolite production [58]. Yesil-Celiktas and coworkers [19] found that cells are large and develop clusters, making them more vulnerable to shear; in addition, the cells become connected while being stirred, and the processing times are extended. In many plant cells cultured in bioreactors, vigorous airflow, blending, and movement promote shearing-related damages, cell wall collapse, aggregation of cellular debris, and polysaccharide production. Cell demise and detritus buildup cause bubbling, leading to the adherence of cells and aggregate to the culture chamber's walls, as well as the creation of a layer on the unit's topmost part; consequently, the circumstances of homogeneous culture are disturbed, resulting in the development of extracellular waste. As the number of cells increases and the cultures become more viscous, greater aeration rates are needed for oxygen delivery and movement. The need for increased oxygenation rates for large-scale growth of plant tissue and cell cultures in bioreactors intensifies foaming and blockage issues [59]. Finally, the irregular production pattern that occurs during subculture usually slows the development of an economic process [60, 61].
Strategies for Solving Constraints
To date, several strategies have been extensively utilized to improve the productivity of secondary metabolites that exhibit bioactive properties in plant cell cultures. Cell culture research and clonal propagation procedures are two significant techniques used in the biotechnological production of plant cells and tissues [19]. Hence, for both research and industry to improve cell culture production and to develop commercially feasible processes, these methodologies should be optimized.
Cell culture investigations began with in vitro callus formation to determine the optimal medium for cultivation. Calli can be collected from any section of a plant that can divide cells. To optimize the creation of a certain molecule, the callus should be initiated from a plant section that has been determined to be an abundant producer [62]. Several factors have been shown to influence the accumulation of secondary metabolites in calli and suspended cells. Numerous recent studies have demonstrated that the nutrient, carbon source, and osmotic stabilizer composition of the culture medium may change to simulate in vitro drought, which can have an impact on metabolic processes and cause the buildup of biomass and secondary metabolites [63]. The most important factors include the chemical makeup of the media utilized in terms of growth promoters; in this respect, the addition of BA and IAA to tissue culture media has a major impact on the distribution and in vitro synthesis of secondary metabolites in Stevia rebaudiana L. [64]. In a different study, it was reported that the generation of secondary metabolites in Zingiber officinale var. rubrum callus culture was increased by picloram [65]. Furthermore, large quantities of proteolytic enzymes from garlic (Allium sativum L.) callus were harvested on MS media supplemented with BAP and NAA [66]. Moreover, naphthaleneacetic acid and picloram produced the best cell suspension cultures for Taxus globosa when added to the Gamborg medium [67].
The carbon source and its concentration, among other important factors, influence the accumulation of secondary metabolites in cell culture [68, 69]. Employing a glucose-fructose mixture or culturing plant tissues in alkanoic acid- or salt-treated media enhanced secondary metabolite productivity and shortened culture time [70]. In another study, paclitaxel synthesis was enhanced by inoculating the cells at a high starting dosage and increasing the saccharide level in the culture medium [71]. The nitrogen source and its concentration also influence the accumulation of secondary metabolites in suspension cultures of different medicinal plants [72, 73]. The influence of nitrogen (N) supply on the rate of cell development, main nutrient intake, and the generation of ginseng saponins and polysaccharides in Panax ginseng cell suspension cultures was investigated, and the results indicated that the proliferation of cells was enhanced by 60 mM N and increased NO3-/ NH4+ ratios. With nitrate alone or in a mixture with ammonium (at a 2:1 ratio) as the N supply, 10 mM N was found to significantly influence the development of cell masses [74]. Growth conditions and environmental stressors, such as excessive heat, salinity, dryness, and light intensity, have also been shown to influence the accumulation of secondary metabolites in calli and suspended cells. Jasmonic acid and methyl jasmonate are important regulators of the formation of secondary metabolites. For instance, plant tissues contain greater amounts of jasmonic acid when pathogens or other stressors are present [75-77].
Light is an essential factor for the building of cell biomass and the production of secondary metabolites. Several studies have shown that light irradiation stimulates the synthesis of substances, such as anthocyanins, in suspension cells [78]. In comparison to dark-grown cultures, light-grown cultures produced more phenolic compounds. However, compared to continuous light-grown suspension cultures, dark-grown cultures produce more flavonoids [79].
In a different report, Cheng et al. [80] showed that in grapevine calluses, light stimulation was necessary for the formation of flavanol, anthocyanin, and flavan-3-ol. Only flavan-3-ol metabolism, particularly trans-flavan- 3-ol production, was positively impacted by increasing light intensity.
Since the early development of plant biotechnology, the effects of temperature on the accumulation of secondary metabolites in suspension cultures have been examined. It has been demonstrated that the proper temperature treatment of suspension cultures is necessary for biomass increase and metabolite synthesis [81].
For clonal propagation techniques, the screening and selection of high-producing cell lines is the initial step. Generally, two approaches are used to select individual cells: single-cell cloning and cell aggregation cloning. The challenges associated with single-cell isolation and culture limit the applicability of this technology. The latter approach appears to be more time-consuming but simpler [82]. This method has been used to produce berberine from the cell culture of Coptis japonica [83]. Choosing and preserving the high-yielding cell line derived from the heterogeneous population of plant cell cultures is necessary because suspensions and callus cultures often provide the desired chemical at first, but after a few passes, the ability to synthesize the product decreases significantly. This decrease in output may be attributed to poor diet or genetic differences. Therefore, the most important strategy for obtaining high-yielding cell lines to synthesize a specific compound is establishing a culture strain from explants obtained from high-yield plants [84].
The immobilization of plant cells is among the manipulative strategies used to encourage secondary metabolite formation, and greater cell-to-cell interactions may lead to increased production [83]. Other reports also indicated that adding precursors improved the accumulation of secondary metabolites [85, 86].
Elicitors are another potential technology used to increase product output in cell culture. Elicitors are parts of plants that trigger signals to activate their chemical defense systems. Several chemical elicitors that have been extensively researched can impact the synthesis of different secondary metabolites and the activation of enzymes in defense systems associated with plants [87]. The recent discovery of this method provides a new route for the synthesis of secondary chemicals [84]. As stated by Nascimento and Fett-Neto [88], plants utilize metabolic pathways that lead to the generation of thousands of secondary metabolites, allowing them to respond successfully to harsh biotic and abiotic conditions. The researchers discovered that the stimulation of secondary metabolism gene expression by injury, herbivore-derived compounds, pathogen elicitors, and oxidative stress induced by heat, drought, flooding, UV light, or high temperatures frequently occurs via the integration of signaling molecules, such as jasmonate, salicylic acid, and their derived compounds. The production of tocopherol in sunflower and Arabidopsis thaliana cell cultures has been successfully increased through the application of jasmonic acid as an elicitor [89]. Other studies have revealed that secondary metabolite yields were significantly increased through innovative, chemically produced elicitors, such as 2-hydroxyethyl jasmonate [90] and 2,6-dichloroINA, a synthetically produced active analog of salicylic acid [91], isonicotinic acid derivatives, and S-methyl benzo- 1,2,3-thiadiazole-7-carboxylate derivative products [92]. In another experiment, the concentrations of Taxol, cephalomannine, and 10-deacetylbaccatin increased after a mixture of the elicitors buthionine sulfoximine and hydrogen peroxide was added [67]. Furthermore, Liang and coworkers [93] reported that Aspergillus flavus, a fungal elicitor, promoted the accumulation of terpenoid indole alkaloids in Catharanthus roseus cambial meristematic cells.
Numerous efforts have been dedicated to enhancing the production of secondary metabolites through genetic engineering [83]. Several secondary metabolites have been developed due to the genetic engineering of microorganisms and plants, in addition to in vitro reconstruction of plant metabolic pathways [94]. These methods include gain-of-function and loss-of-function strategies, which have been implemented with unique genes [95]. In addition, the expression of transporters in cultured plant cells also demonstrated the ability to transport hazardous substances from the plant cell to the extracellular environment [96].
Cell metabolic engineering, a natural type of recombinant DNA, is another technique used to increase the productivity of plant cell cultures. In a broader manner, metabolic engineering can create biochemical reaction pathways to increase the rate of a desired product, decrease the rate of undesirable byproducts, or break down harmful or undesirable chemicals [97]. Agrobacterium-mediated transformation has been used in metabolic engineering to increase the production of secondary metabolites in vitro or by introducing a foreign gene [98].
Moreover, metabolic engineering of plant secondary metabolite pathways has potentially provided an intriguing new approach for increasing the output of commercially relevant chemicals in plants or plant cell cultures or even for producing entirely novel compounds [99]. For instance, the shikimate pathway and the isoprenoid pathway can be bioengineered to biosynthesize aromatic chemicals in plants [100, 101]. Similarly, metabolic engineering can be applied to certain functional groups that act as markers for specific secondary products generated by plants, such as sesqui-, di-, and triterpenes, monoterpenoids, and carotenoids.
Metabolic inhibitors, elicitors, and precursors were used to investigate the pattern of taxane synthesis and metabolic pathway compartmentation in Taxus chinensis cell cultures [102]. The yield-limiting factors were identified, which aided in the metabolic engineering of Taxus cell cultures for paclitaxel synthesis. In a different study, when two genes encoding tryptophan decarboxylase and strictosidine synthase were isolated from Catharanthus roseus and inserted into tobacco, cells generated strictosidine after being supplied with secologanin [103]. Shinmyo and colleagues [104] created a gene expression system for the metabolic engineering of cultivated tobacco cells by isolating three cDNA clones with high mRNA levels at the stagnant growth stage. The authors argued that these gene promoters could be useful for promoting gene expression in high-density cell cultures.
Knowledge of the biosynthetic pathways that generate desirable phytochemicals in plants and cultures remains limited, necessitating efforts to develop information at both the molecular and cellular levels [105]. In this approach, the identification of transcription factors that can control the complete pathway has provided new options for the regulated generation of secondary metabolites. Yun and colleagues [106] demonstrated that introducing a gene encoding hyoscyamine-6- hydroxylase, which was originally found in Hyoscyamus niger, into Atropa belladonna enabled the manufacture of the valuable tropane alkaloid scopolamine, which was previously detected at only small levels in A. belladonna. Almost all the hyoscyamines were transformed into scopolamine. This was likely the first practical example in which a valuable medicinal plant was genetically engineered to yield a profitable product. An excellent example is the production of podopyllotoxin, the precursor of a semisynthetic anticancer medication, via biotransformation caused by the addition of coniferin to a Podophyllum hexandrum suspension culture.
The growing commercial importance of plant-derived secondary metabolites has sparked interest in large-scale manufacturing, especially the ability to modify the synthesis of bioactive metabolites using cell culture technology [107]. Bioreactors provide ideal conditions for large-scale plant production for commercial purposes. As a result, much work is now being devoted to developing novel bioreactor designs. To manage plant morphogenesis and biomass production in bioreactors, various culture variables, such as morphology, oxygen supply, and CO2, must be monitored and/or regulated. According to Yesil-Celiktas et al. [19], optimizing the scale-up of plant cell and tissue cultures requires a complete understanding of substrate needs and culture conditions. Carbon and oxygen are two primary substrates that influence biomass production; hence, their utilization rates should be regularly monitored.
Table 2.
Secondary metabolites obtained from plant suspension cultures along with their uses and economic value.
The physical conditions within the reactor interact with the chemical conditions, affecting both costs and productivity efficiencies. Efforts to control contamination in liquid cultures have been made by creating the ElecTIS single-container TIS bioreactor prototype. The primary advantages of this new TIS bioreactor are its simplicity of use, the steady reduction in the risk of contamination resulting from forced insufflation of outside air in traditional bioreactors, and a greater rate of multiplication compared to traditional cultures in a gelled medium [108].
The use of plant cell culture as a manufacturing approach is becoming increasingly important as customer demand for natural products and additives grows [109]. Furthermore, expanded medicinal applications, such as phytotherapy, may increase the industrial use of plant cell culture.
As genetic manipulations of cell cultures can change the metabolic profile of plants, industrial efficiency is projected to increase in the future [110].
Finally, functional genomics techniques (transcriptomics, proteomics, and metabolomics) are effective methods for expediting thorough examinations of biological processes, which in turn quicken the gene discovery process for secondary metabolite pathways and boost secondary metabolite output. These approaches include the use of two-dimensional gel electrophoresis-based proteomics and transcript analysis techniques, such as differential display, EST databases, and microarrays, to examine the production of certain secondary metabolites [111].
Economic Benefits and Prospects
Despite developments in the organic synthesis or semi-synthesis of a wide range of molecules equivalent to those produced by plants, the extraction of bioactive compounds from plants remains commercially important [112] (Table 2).
In general, plant compounds of commercial importance are secondary metabolites, which are divided into three categories: essential oils, glycosides, and alkaloids [113]. Essential oils are a blend of terpenoids that are utilized as flavoring agents, fragrances, and solvents. Glycosides include flavonoids, phenolics, tannins, saponins, cyanogenic glycosides, and mustard oils, which are used as dyes, food coloring agents, and pharmaceuticals (e.g., steroid hormones, antibiotics, and digitalis) [114]. Alkaloids are a varied collection of chemicals with approximately 4000 recognized structures; nearly all naturally occurring alkaloids are of plant origin. Alkaloids (e.g., morphine, cocaine, strychnine, and nicotine) are physiologically active in humans and very important to the pharmaceutical industry [115]. Many of these metabolites are difficult or impossible to manufacture at reasonable costs. Furthermore, in certain circumstances, consumers prefer natural products to artificially generated products.
The growing commercial value of secondary metabolites has led to increased attention on secondary metabolism in recent years, especially regarding the possibility of modifying the synthesis of bioactive plant metabolites using cell culture technologies [23]. Plant cell culture shows great potential for the in vitro production of complex secondary metabolites [116]. Plant cells have recently received increased attention for their ability to generate natural or recombinant chemicals of economic significance [117]. This is primarily due to its economic, scalability, and safety advantages over conventional microbial and mammalian production methods [19]. Plant-derived bioactive compounds are being used as medicines, agrochemicals, taste and fragrance components, food additives, and pesticides [24]. There has been a renewed interest in natural products worldwide. The market for natural plant goods has grown quickly in recent years, and this pattern is expected to continue because more consumers prefer natural compounds [118]. With technical improvements, plant cell culture will continue to contribute to the market in the future. The global market for plant-derived compounds, such as medications, perfumes, flavors, and color components, exceeds several billion dollars each year [119].
Bioreactors are perfect for mass-producing plants for commercial purposes. Much work has recently been performed to optimize these systems for the synthesis and recovery of high-value medicinal plant components, including ginsenosides and shikonin. Conventional methods utilize the bark of 100-year-old trees to be harvested to acquire 1 kg of the active component Taxol. In the past two decades, researchers have developed effective procedures for extracting cell cultures and large-scale bioreactor technology. The acceptability of this procedure for the industrial manufacturing of this priceless molecule was newly found, and it will have significant effects on the production of tumor-inhibiting medication. Recent advancements in plant cell culture, molecular biology, fermentation technology, and enzymology indicate that these systems will become achievable sources of critical secondary metabolites. Furthermore, advances in plant cell metabolic engineering, such as significant enhancements in cell physiology and secondary metabolism, may increase the efficiency of several plant cell activities and propel them to a profitable, viable phase for the commercial manufacturing of beneficial metabolites. Close collaboration between biologists and biochemical engineers will soon be needed, requiring scholars in both fields to broaden their knowledge bases and study fields to hybrid cutting edges.
Conclusion
There are clear advantages of plant cell cultures for the generation of secondary metabolites compared to traditional techniques, including the ability to produce relevant metabolites under controlled conditions, independent of environmental factors; the ability to optimize culture conditions to increase the production of secondary metabolites; the ability to obtain healthy and disease-free plant material; and the ability to cultivate any plant in vitro, regardless of whether it has tropical or subtropical origins. Moreover, recent advances and developments in metabolic engineering and recombinant DNA technology may provide an efficient system for in vitro production of secondary metabolites by manipulating the enzymes of a metabolic pathway in plant cell cultures. Thus, the method may provide new means to produce disease-remediating or disease-controlling molecules at low costs, which would benefit humanity. Therefore, biotechnology should be further advanced, which could be achieved by strengthening and funding research programs.

