

Introduction
With the rapid development of the coffee and tea industries, large quantities of coffee grounds and oolong tea waste are produced worldwide each year. Traditionally, these waste materials were disposed of through methods such as dumping, incineration, and landfilling as part of municipal solid waste management [1]. However, these handling methods are unable to meet the sustainable development goals for organic solid waste disposal due to the production of highly polluted leachate and significant greenhouse gases emissions, leading to a negative impact on environmental quality [2, 3]. Furthermore, coffee grounds and oolong tea waste contain abundant nutrients and bioactive components that are underutilized, leading to significant resource wastage [4-6]. Similarly, camphor leaves, a substantial component of garden waste, are often discarded and their inherent value remains untapped [7]. In light of these environmental concerns and the need for effective resource utilization, composting has gained significant attention in recent years. Composting is considered one of the most suitable options for managing and treating solid organic waste, as it facilitates nutrients cycling and promotes the reuse of organic fractions, thereby reducing pollution and environmental impact [8].
Commonly known as edible roses, Rosa rugosa (Rosales: Rosaceae) is a significant cash crop cultivated using facility cultivation techniques, which have improved the growing conditions of the crop, while also introducing certain challenges [9]. Continuous monocropping of the same crop can disrupt the soil nutrient balance, leading to the depletion of specific nutrients. Consequently, this can lead to the proliferation of certain microorganisms, an increase in pathogenic populations, and a corresponding decrease in beneficial bacterial species and their abundance [10-12]. Such impacts not only affect the normal growth of crops but also have adverse effects on the quality and yield of agricultural products, thereby diminishing the economic benefits [13]. Therefore, it becomes crucial to implement appropriate measures to enhance the fertility of facility soil.
.
Numerous studies have consistently demonstrated the efficacy of compost products in enhancing soil fertility. By incorporating an appropriate amount of compost products into the soil, which are rich in high-quality organic matter and readily available nutrients, the supply capacity of essential elements such as nitrogen, phosphorus, potassium, and organic matter can be significantly improved [14, 15]. The core process of composting involves the enzymatic hydrolysis of organic matter, which stimulates microorganisms to secrete enzymes such as cellulase, sucrose, and protease. These enzymes play a crucial role in breaking down organic matter in the soil, releasing nutrients that can be easily absorbed by plants. Furthermore, they contribute to the cycling and utilization of nutrients within the soil [16, 17].
Vermicomposting, a widely practiced technique for soil fertility improvement, has been found to yield compost products with higher levels of both macronutrients and micronutrients compared to regular compost derived from the same raw materials. The inclusion of earthworms in the composting process promotes organic matter decomposition, increases soil enzyme activity, and enhances soil microbial biomass [18, 19], and creates a favorable growth environment for crops. Previous research has also highlighted the benefits of earthworm composting in addressing soil fertility issues associated with continuous cropping. For example, Zhao et al. [20] discovered that earthworm composting enhanced the fertility of greenhouse tomato soil subjected to continuous cropping pressures, effectively mitigating the adverse effects of secondary salinization and alkalization. Ding et al. [21] reported that the application of urban garbage earthworm compost significantly improved soil quality and countered degradation resulting from continuous watermelon cultivation. However, there is a lack of research on composting to improve soil for the continuous cultivation of roses.
To address the pressing issues of urban waste management and promote the resource utilization of these wastes, this study focused on investigating the effects of in-situ earthworm compost on soil used for continuous cropping rose. Vermicompost primarily consists of plant materials, and its nutrient content varies depending on the composting materials utilized, thereby offering diverse effects on soil improvement. In this context, the aim of this research is to explore the potential of earthworm composting using different organic materials, such as coffee grounds (T1), camphor leaves (T2), and oolong tea waste (T3), and analyze the feasibility of using various waste materials to improve the soil used for continuous cropping of rose. The study specifically focused on examining the effects of earthworm composting on the chemical properties and bacterial community structure of protected rose soil. The primary objective was to establish scientific evidence supporting the use of earthworms in mitigating the degradation of continuously cropped rose soil. Additionally, the study aimed to investigate the interplay between soil microorganisms, soil chemical properties, and soil enzyme activity, with the ultimate goal of gaining valuable insights into addressing the challenges of soil degradation resulting from continuous cropping through composting.
Experimental Methods
Experimental Materials and Earthworm Breeding
The organic materials utilized in this experiment consist of coffee grounds sourced from Luckin Coffee, camphor tree leaves collected from Guanshatian Road, Wuyi University, and oolong tea waste obtained from the waste generated during oolong tea production at the College of Tea and Food Science in Wuyi University. The specific earthworm species employed in this study was Eisenia foetida Savigny, with the rearing method following the approach outlined by Huo et al. [22]. The earthworms were cultivated in black storage boxes measuring 350×256×125 mm, with soil moisture levels maintained at 20%-30% and an indoor temperature at 25±1ºC.
Soil Sample Collection and Processing
The soil used in this study was obtained from the greenhouse at Wuyi University. This particular soil had been continuously utilized for cultivating edible roses for a duration of 5 years. For Treatment 1 (T1), a mixture of 500 g of coffee grounds and 1500 g of soil was prepared and thoroughly blended. Similarly, for Treatment 2 (T2), 500 g of camphor tree leaves were evenly mixed with 1500 g of soil. For Treatment 3 (T3), 500 g of oolong tea waste was combined with 1500 g of soil. The control group (CK) solely consisted of 2000 g of soil without any additives.
After introducing the earthworms into soil amended with various organic waste materials, soil samples were collected after 30 days of cultivation using a five-point sampling method. The soil samples were collected from a depth of 25-125 mm at each treatment using a soil sampler, and the samples from five distinct points were combined thoroughly. Each treatment was replicated three times.
Following air drying, each soil sample was divided into two parts. The first part, weighing 500 g, was stored at 4ºC to facilitate the subsequent analysis of soil physicochemical properties, such as soil enzymes, organic matter, available phosphorus, available nitrogen, and available potassium. The second part, weighing 10 g, was stored at -30ºC and then sent to Shanghai Personalbio Biotechnology Co., Ltd. for DNA extraction, amplification, and high-throughput sequencing analysis. This study aimed to determine the diversity and composition of soil bacteria.
Determinations of Soil Chemical Properties and Enzyme Activity
Soil samples were sieved using a 100-mesh sieve for the determination of soil chemical properties. The organic matter content in the soil was measured using the potassium dichromate titration method [23]. The available nitrogen (AN) was determined using the alkaline diffusion method. The available phosphorus (AP) was measured using the molybdenum-antimony colorimetric method with 0.5mol/L NaHCO3 extraction [24, 25]. The available potassium (AK) was determined using the ammonium acetate extraction-flame photometry method [26]. Five soil enzymes were analyzed, including soil acid protease, soil neutral protease, soil alkaline protease, soil cellulase and soil sucrase. Protease activity was determined using the Folin-phenol method [27]. Soil cellulase activity was determined using the anthrone colorimetric method, and soil sucrase activity was determined using the 3,5-dinitrosalicylic acid method [28, 29].
Extraction of Total DNA from Soil
We used the DNeasy PowerSoil Kit from Mo Bio/ QIAGEN to extract DNA, and the extracted DNA was then tested. The DNA concentration was determined by measuring the absorbance at 260 nm and 280 nm using a fluorescence spectrophotometer (Quantifluor-ST fluorometer, Promega, E6090; Quant-iT PicoGreen dsDNA Assay Kit, Invitrogen, P7589). The quality of the DNA was assessed using a 1% agarose gel electrophoresis. The concentration of the DNA solution was adjusted, and the working DNA solution was stored at 4ºC, while the storage solution was kept at -20ºC.
High Throughput Sequencing Analysis of 16S rDNA
Firstly, the 16S rRNA variable region was amplified. A PCR pre-experiment was performed to target the specific V region of the sample DNA. Next, a large-scale PCR amplification was carried out using Pyrobest DNA Polymerase from TaKaRa (DR500A). Subsequently, gel extraction and purification were performed by targeting the desired bands to obtain purified samples employing the AxyPrep DNA Gel Extraction Kit from Axygen (AP-GX-500). Afterward, quantification of each sample was conducted using the BioTek enzyme marker. Finally, the required on-machine sequencing was performed by adopted the standard Illumina TruSeq DNA library preparation experimental process as outlined inthe llumina TruSeq DNASample Preparation Guide.
Data Analysis
In this study, one-way analysis of variance (ANOVA) using SPSS 26.0 software was employed to evaluate the differences in soil chemical properties across different organic materials. The LSD test was performed with a significance level of P<0.05 to identify significant differences between groups. Furthermore, a correlation analysis was conducted to examine the relationship between differential bacterial species and soil chemical properties. For taxonomic composition analysis and to generate a rarefaction curve, QIIME2 (2019.4) was used. Box plots for the Chao1 and Shannon diversity indices were created using GraphPad Prism 8. Relative abundance plots at the phylum and genus levels, based on the Bray-Curtis distance matrix, were generated using the ggplot2 package in R 4.3.1. NMDS analysis was performed, and a two-dimensional sorting plot was created to visualize the composition differences in microbial communities. To create an OTU Venn diagram, the VennDiagram package in R 4.3.1 was employed. PCA clustering analysis was conducted using the Vegan package. Canoco 5 software was used to perform redundancy discrimination analysis (RDA), the Python LEfSe package was utilized for Linear discriminant analysis Effect Size (LEfSe) analysis, and TBtools was employed to generate correlation heatmaps.
Results
Effects of Cultivating Earthworms in Different Organic Substrates on Soil Nutrition and Enzyme Activities
According to the results shown in Table 1, significant differences were observed in soil nutrient content and soil enzyme activity among different composite matrices. The available potassium and organic matter in T1 and T2 were significantly higher than those in the CK group. Similarly, T3 exhibited significantly higher levels of available nitrogen, available potassium, and organic matter compared to CK group. However, no significant difference in available phosphorus was observed between the three experimental groups and the control group. Regarding soil enzyme activity, there was no significant difference in soil acid protease, soil neutral protease, and soil sucrase among the three experimental groups compared with the CK group. However, soil cellulase activity was significantly higher in the experimental groups compared to the CK group. Additionally, the alkaline protease activity in T2 and T3 was significantly higher than that in the CK group. Based on the statistical differences observed in multiple soil indicators after adding oolong tea waste to earthworms, it can be concluded that oolong tea waste has a significant impact on soil nutrition and soil enzyme activity compared to coffee grounds and camphor tree leaves.
Effects of Cultivating Earthworms in Different Organic Substrates on Soil Bacterial Diversity
To evaluate the soil bacterial communities, a high-throughput 16S rDNA amplicon sequencing approach was employed. The dilution curve demonstrated that the sequencing depth achieved was adequate to cover the majority of bacteria in the samples (Fig. 1a). The Chao1 and Shannon indices were utilized to assess the impact of the interaction between the three substrates and earthworms on the abundance and diversity of soil bacteria (Fig. 1(b, c)). Specifically, the abundance of bacterial communities in T1 and T2 exhibited a significant increase when compared to the control group (CK). However, the impact on the diversity of soil bacterial communities was relatively moderate. Based on the coverage estimation, which exceeded 0.96 for soil bacteria, it can be inferred that the sequencing depth effectively captured the true bacterial composition in the soil samples.
Table 1.
Soil chemical properties and enzyme activities in earthworm-incubated soil with various organic materials.
[i] AN: available nitrogen, AP: available phosphorus, AK: available potassium, OM: organic matter, ACPT: acid protease, NPT: neutral protease, ALPT:alkaline protease, CL:cellulase, SG: sucrase T1: earthworm+Coffee grounds: T2: earthworm+Camphor tree leaves; T3: earthworm+Oolong tea yellow tablets; CK: Untreated garden soil. The values in the table were mean ± standard deviation, and those with different lowercase letters after the values in the same row indicate significant differences (LSD test, P<0.05, n = 3).
Fig. 1.
Rarefied fraction curves a), Chao1 index b), Shannon index c), PCA analysis d) and NMDS analysis e) of the bacterial community in rose soil following earthworm incubation with various organic substrates.
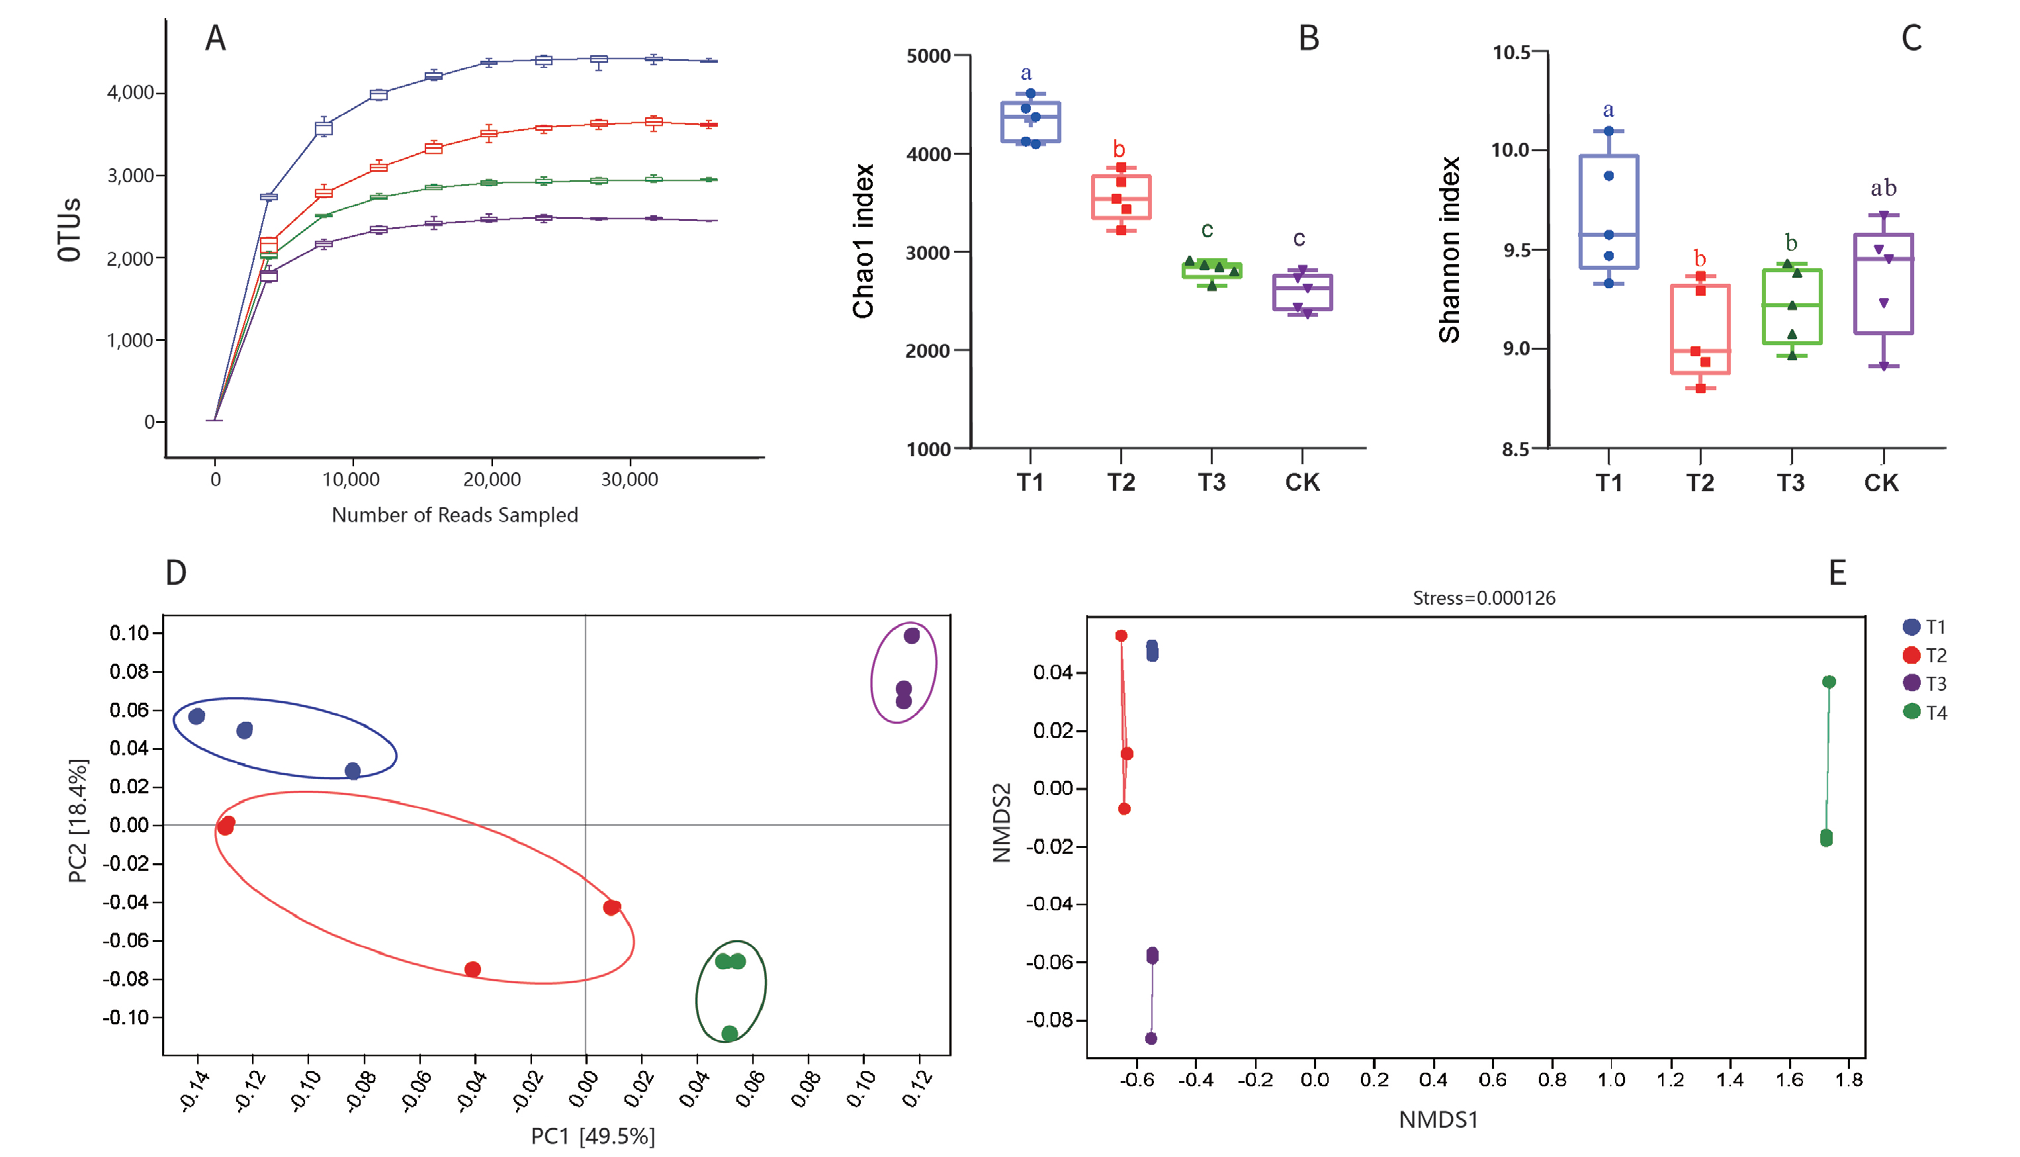
Based on the Euclidean distance algorithm, beta diversity analysis was employed to assess the differences in bacterial communities. The PCA plot clearly demonstrated distinct variations among bacterial communities in the different treatment groups, as each group appears to be distributed in a distinct quadrant. This observation suggested significant dissimilarities in the composition of bacterial communities between the various treatment groups. To further investigate the dissimilarities in soil bacterial community structure among the different treatments, non-metric multidimensional scaling (NMDS) was performed (Fig. 1e). The soil bacterial community structures of T1, T2, and T3 were found to be significantly different from the control (CK), with T1 group exhibiting relatively strong group consistency. These results indicated that the interaction between earthworms and different substrates can induce changes in soil microbial community structure. Furthermore, the addition of coffee grounds had a more pronounced impact on soil microorganisms when compared to oolong tea waste or camphor tree leaves.
Comparisons of Soil Bacterial Community Composition, Community Structure, and Species Composition under Different Treatments
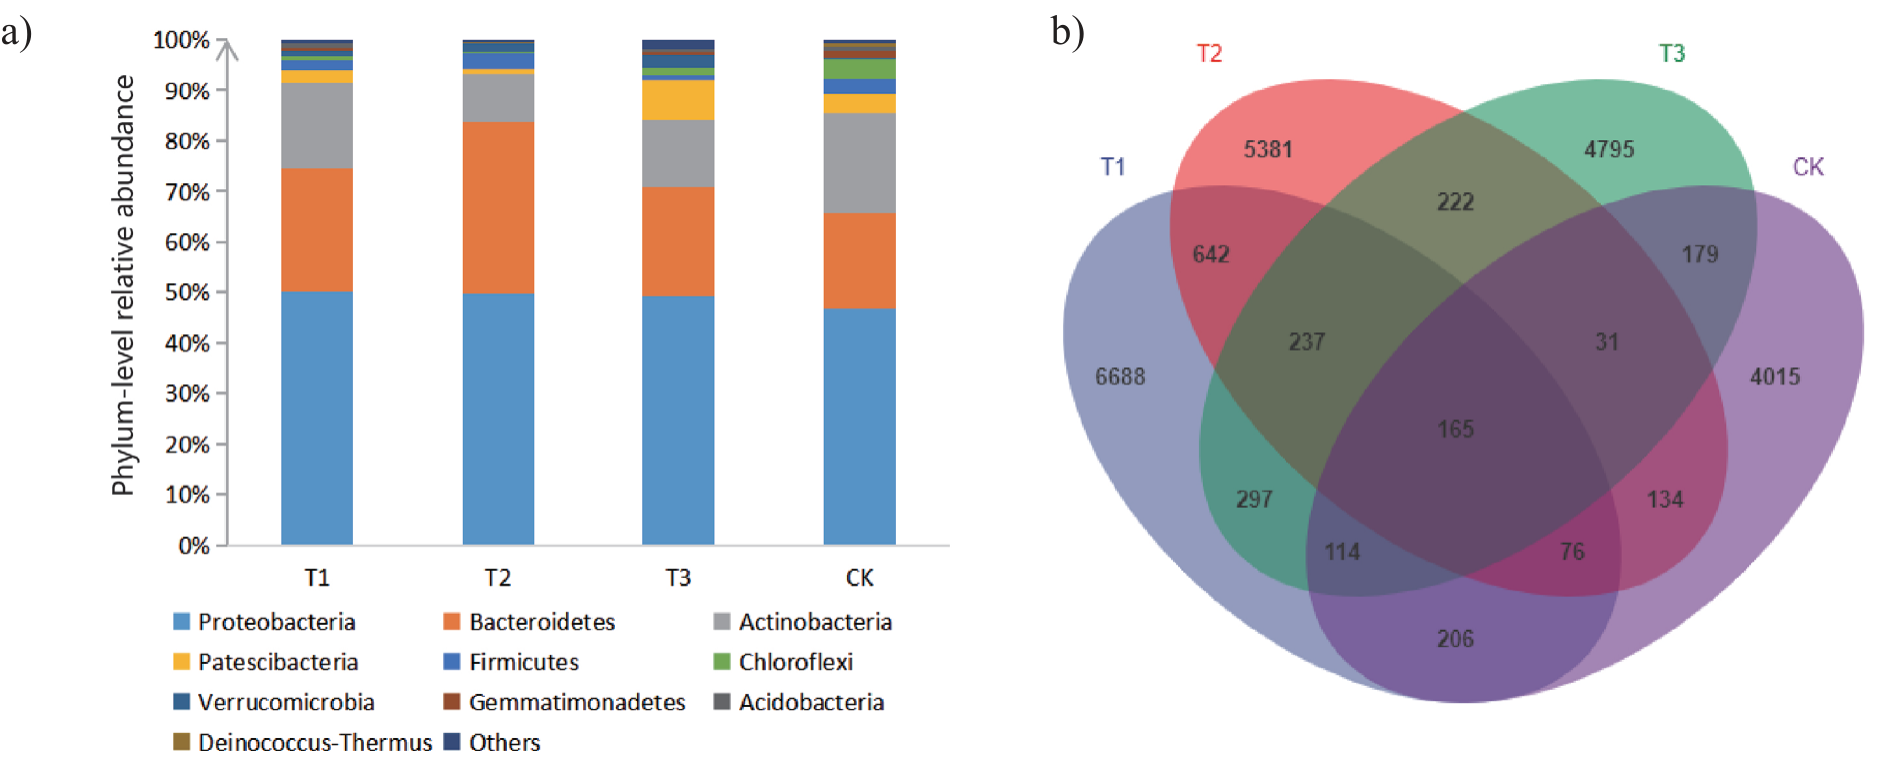
According to a study examining the bacterial phylum level, the dominant bacterial phyla in all experimental groups were Proteobacteria, Bacteroidetes, and Actinobacteria, with relative abundance of over 85% and a maximum of 95%. Furthermore, there was no significant difference observed between the four groups (Fig. 2a). These findings suggested that the soil bacterial community remained relatively stable at the phylum classification level despite the different substrate treatments. In comparison to the control group (CK), there were no significant differences in the relative abundance of Proteobacteria among all treatment groups. However, the relative abundance of Bacteroides increased in all treatment groups, with T2 showing the most significant increase. The relative abundance of Actinobacteria increased in T1 and T3, while T2 exhibited the most substantial decrease. Additionally, compared to CK, the relative abundance of Patescibacteria decreased to varying degrees, while the relative abundance of Firmicutes increased to varying degrees in the three treatments. However, the Venn diagrams showed that specific soil bacteria were affected by different substrate treatments.
Based on the Venn diagrams (Fig. 4d) , it was observed that the total number of soil bacterial operational taxonomic units (OTUs) was 17,788. Among the different treatment groups, T1 obtained 6,688 OTUs, T2 obtained 5,381 OTUs, T3 obtained 4,795 OTUs, and the control group (CK) obtained 4,015 OTUs. Only 165 OTUs were shared by all soil bacteria, which accounted for a mere 0.9% of the total. The endemic OTUs for T1, T2, T3 and CK groups were 4,951, 3,847, 3,550 and 3,110 respectively. These findings indicated that the presence of earthworms significantly improves the diversity of bacteria in the soil. Fig. 2 further supported this observation by illustrating that the total number of OTUs in the treatment group was higher compared to the CK group. Furthermore, the bacterial OTUs in the T1 group were significantly higher compared to the T2 and T3 groups. Overall, the introduction of different substrates to earthworms resulted in an increased number of bacterial OTUs in the soil, with T1 demonstrating the most favorable effect.
Fig. 2.
a) Phylum-level relative abundance of soil bacteria in the interacted rose soils incubating earthworms in different substrates. b) Venn diagrams showing the overlap of core operational taxonomic units (OTUs) among soil bacteria in the different treatment groups.
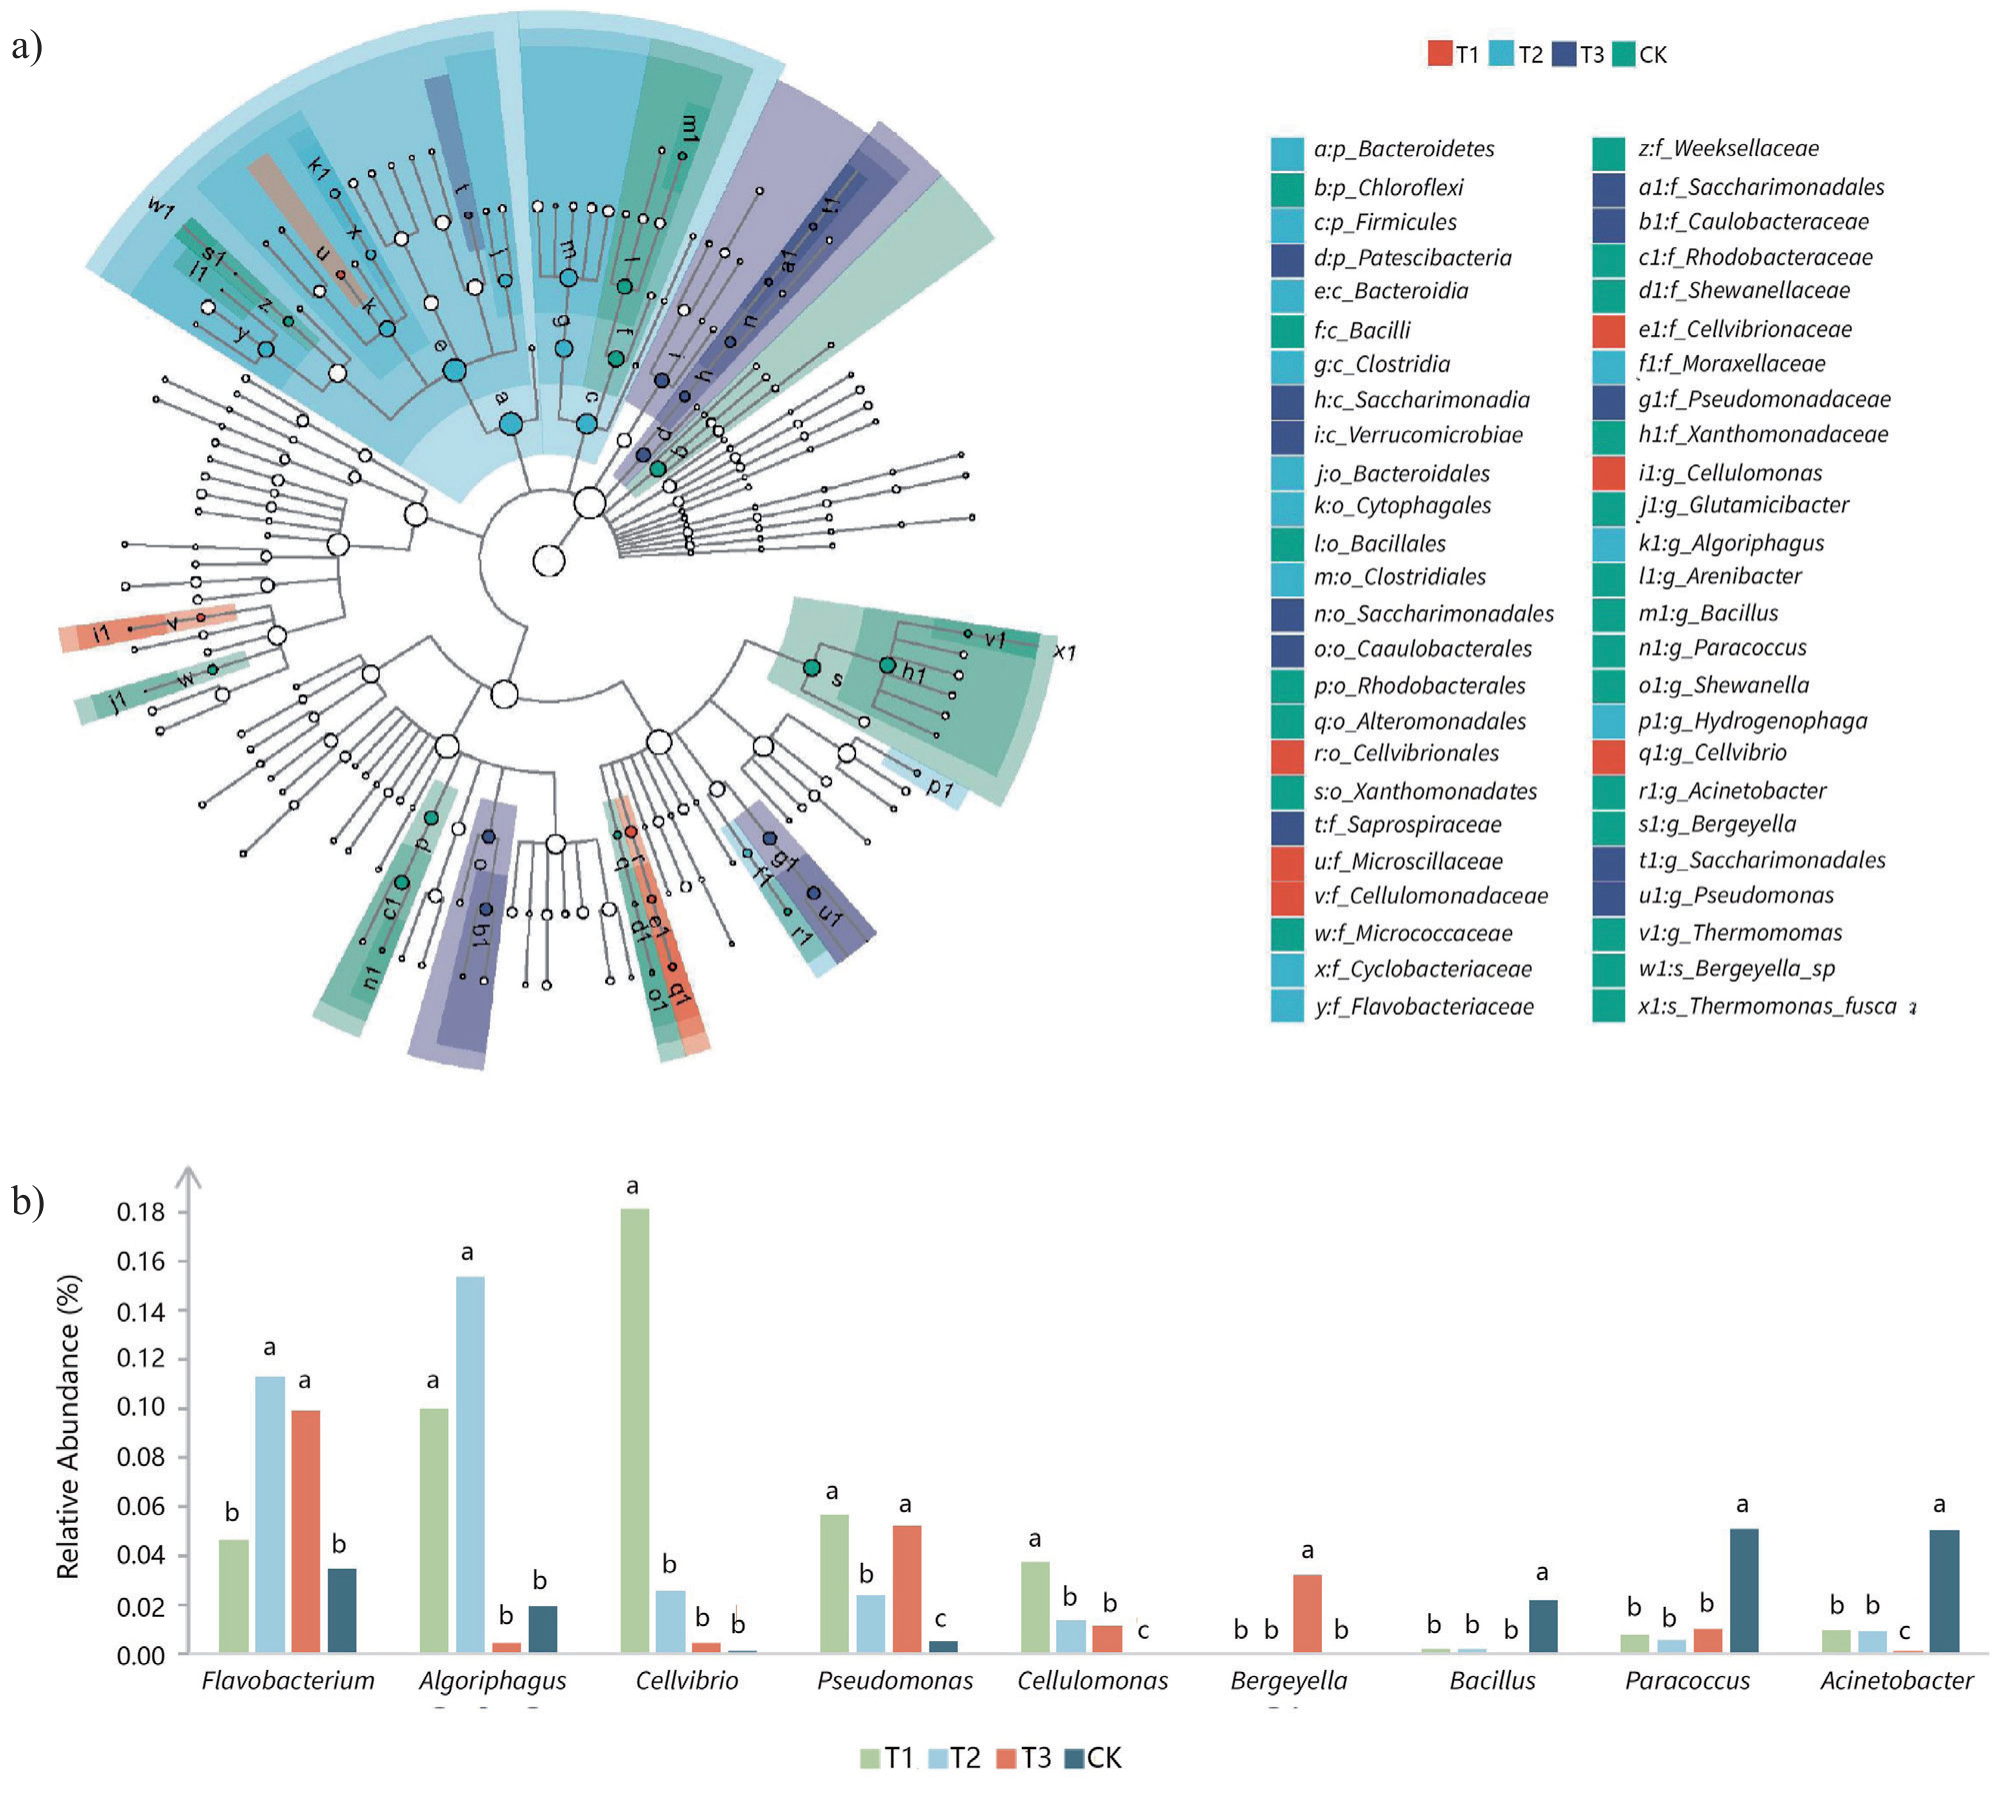
No significant differences were found at the phylum level among the four groups. To identify OTUs with statistically significant differences between the sample groups. LEfSe analysis was performed. The branch plot (Fig. 3a) displayed the core microorganisms with LDA values greater than or equal to 4. Based on the LEfSe analysis of four groups of bacteria, a total of 50 taxa were enriched, including four phyla and 16 genera. T1 exhibited enrichment in six taxa, including two genera; T2 showed enrichment in 12 taxa, including Bacteroidetes and Firmicutes at the phylum level and two genera; T3 displayed enrichment in 11 taxa, including the phylum Patescibacteria and two genera; and CK demonstrated enrichment in 21 taxa, including the phylum Chloroflexi and 10 genera.
Integrating with the genera-level relative abundance diagram of bacteria (Fig. 3b), it was evident that when compared to the CK group, the T1, T2 and T3 groups exhibited significantly upregulation in five genera, namely Algoriphagus, Cellvibrio, Pseudomonas, Cellulomonas, Pseudoxanthomonas. Conversely, these three groups showed substantial downregulation in the expression of three genera, including Bacillus, Paracoccus, and Acinetobacter.
The relative abundance analysis revealed that Flavobacterium, Algoriphagus, Cellvibrio, and Pseudomonas were more abundant in all experimental groups. Among the three treatment groups (T1, T2, and T3), the most dominant strain was Cellvibrio in T1, Algoriphagus in T2, and Flavobacterium in T3. In contrast, the most dominant strain in CK group was Pseudomonas. Comparing the treatment groups with CK, there was an increase in the relative abundance of Flavobacterium, Algoriphagus, Cellvibrio, Pseudomonas, and Cellulomonas. On the other hand, the relative abundance of Bacillus, Paracoccus, and Acinetobacter decreased in the treatment group.
Indeed, the relative abundance of Algoriphagus and Cellvibrio increased the most in T1 compared to CK. Similarly, in T2, the relative abundance of Flavobacterium, Algoriphagus and Cellvibrio showed the highest increase compared to CK. In T3, the most significant increase in relative abundance was observed for Paracoccus, Acinetobacter and Castellaniella. This overall pattern suggests that the introduction of different organic matter by earthworms led to varying degrees of changes in the genus-level composition of bacteria. The specific bacterial genera mentioned above exhibited notable alterations in their relative abundance, indicating their potential roles in responding to and utilizing the introduced organic material.
Correlation Analysis between Bacterial Abundance and Soil Nutrients
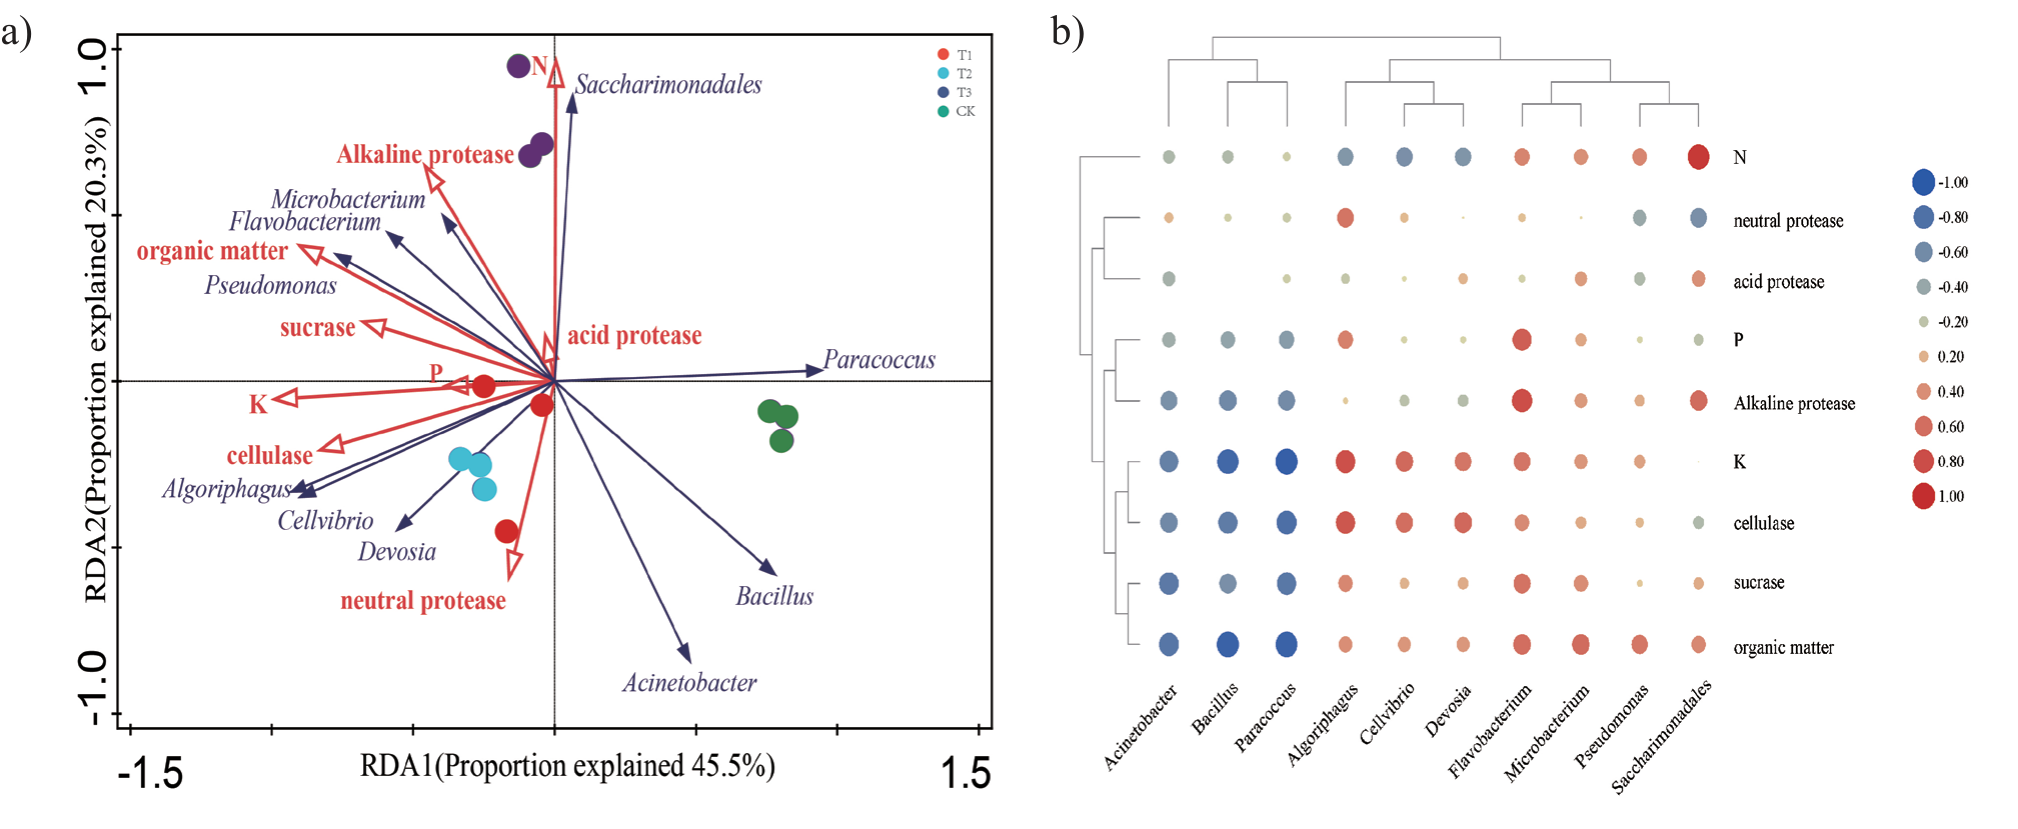
Redundancy analysis (RDA) was used to investigate the relationship between soil nutrients, soil enzyme activity, and soil bacteria. The results showed that alkaline protease exhibited a positive correlation with available nitrogen and organic matter. Moreover, sucrase and cellulase demonstrated positive correlations with available phosphorus, available potassium, and organic matter. On the other hand, neutral protease displayed a negative correlation with available nitrogen. Furthermore, different bacterial genera were found to be enriched in specific environmental conditions. By examining the distribution of soil bacterial sample points in Figure 4-A, it was evident that T1 and T2 are distributed in one area, while T3 and CK are respectively distributed in the other two areas, exhibiting distinct regional distributions, and indicating that different treatments had a significant impact on soil nutrients, soil enzyme activity, and microbial community structure. The relative abundance of beneficial bacteria in the soil demonstrated a positive correlation with T1, T2, T3, while showing a negative correlation with CK. These findings indicated that the interaction between earthworms and different substrates can effectively enhance the structure of soil bacterial communities.
Fig. 3.
LEfSe analysis and relative abundance of significantly different bacterial taxa in the interacted rose soils incubated with earthworms using different substrates. a) LEfSe analysis (LDA score>4) depicting the bacterial taxa that showed significant differences in relative abundance among the treatment groups. b) Bar chart displaying the relative abundance of the significantly different bacterial genera identified in the interacted rose soils incubated with earthworms using different substrates.
Correlation analysis revealed significant differences in bacterial genera in relation to soil nutrients and enzyme activities (Fig. 4b). The genera of Flavobacterium, Algoriphagus, Cellvibrio and Pseudomonas exhibited positive correlations with soil nutrients such as available potassium, alkaline protease, cellulase, and soil organic matter. Notably, Flavobacterium showed a highly significant positive correlation with alkaline protease, while Algoriphagus demonstrated a highly significant positive correlation with available potassium and cellulase (P<0.01). Furthermore, Cellvibrio exhibited a significant positive correlation with available potassium and cellulase (P<0.05). On the other hand, the genera Bacillus, Paracoccus and Acinetobacter displayed a negative correlation with overall soil nutrients levels. These bacterial genera were most impacted by factors such as available potassium, sucrase, cellulase, and organic matter, showing a highly significant negative correlation. Specifically, available potassium, alkaline protease, cellulase, and organic matter demonstrated strong positive correlations with the genera Flavobacterium, Algoriphagus, Cellvibrio and Pseudomonas, while showing strong negative correlation with the genera Bacillus, Paracoccus and Acinetobacter. Based on these findings, it can be deduced that available potassium, alkaline protease, cellulase and organic matter are key factors influencing soil bacterial abundance under different substrate treatments.
Discussion
Improving Soil Nutrition and Enzyme Activities through Cultivating Earthworms in Various Organic Substrates
Based on previous researches [30-32], we have chosen specific soil chemical indicators (AN, AP, AK, OM) and soil enzyme activity indicators (ACPT, NPT, ALPT, CL, SG) that are closely associated with soil fertility and can effectively reflect the impact of different treatments on soil fertility. In our experiment, we utilized camphor tree leaves, coffee grounds, and oolong tea waste as substrates in conjunction with earthworms. This combination resulted in an enhanced nitrogen (N) and potassium (K) supply capacity of the soil, as well as an increase in organic matter content. Organic matter is a vital component of the soil environment, as it undergoes mineralization to release a significant amount of nutrients, providing nourishment for plant growth. It also serves as the primary source of available nitrogen (N) and phosphorus (P) for plants. Although fertilization practices may impact the physicochemical properties of soil when cultivating edible roses over long term, it is generally observed that the nitrogen (N) and potassium (K) content decreases after each harvest due to the removal of aboveground flower parts. However, a significant amount of phosphorus (P) tends to remain in the soil [7]. The results of this experiment demonstrate that using the in-situ composting with earthworms and oolong tea waste effectively increases the nitrogen (N) and potassium (K) content in soil planted with roses. However, the content of phosphorus (P) does not show significant changes.
Soil enzymes play a crucial role in soil material cycling and nutrient supply [33]. They contribute to the transformation of soil materials and energy metabolism, and aid in the degradation of external organic matter, which is critical for ecosystem functioning. Out of the five enzymes measured in this experiment, only soil alkaline protease and soil cellulase exhibited significant changes. Soil cellulase, in particular, plays a key role in carbon cycling by producing glucose as the final product [34]. Protease is involved in the transformation of amino acids, proteins, and other nitrogen-containing organic substances in the soil. Its hydrolysis products serve as a nitrogen source for higher plants [35]. The increase in the content of these two enzymes accelerates nutrients cycling and utilization in the soil, thereby enhancing its self-repair capacity [36].
Earthworms play a crucial role in the decomposition of organic materials by utilizing their feeding behavior and digestive tract. This process involves the presence of enzymes such as amylase, protease, and cellulase within their gizzard, leading to biochemical reactions [37, 38]. As a result, these materials undergo a breakdown process and transform into simple carbohydrates, which then combine with soil minerals to form organic or inorganic complexes. The selected experimental substrates like coffee grounds, camphor tree leaves and oolong tea waste exhibit a slightly acidic nature. Our findings indicate that introducing earthworms during the composting process helps to neutralize organic acids, thereby promoting pH neutralization. This neutralization occurs through the secretion of calcium or carbonates by the calcium glands located in their digestive tract. As a result of earthworm activity, the composting process achieves a more neutral pH. This is highly advantageous as it creates favorable conditions for the growth and reproduction of microorganisms and plants [39, 40]. Compared to ordinary composting methods, incorporating earthworms significantly enhances the overall quality of the compost by neutralizing organic acids and providing an environment conducive to microbial and plant growth.
The experimentation yielded compelling results, highlighting the positive impact of introducing earthworms to specific organic matter on soil chemical properties and soil enzyme activity. Among the three substrates tested, oolong tea waste and coffee grounds displayed superior outcomes. Particularly, the oolong tea waste exhibited a more pronounced effect on enhancing soil enzyme activity in comparison to coffee grounds.
Exploring Variations in Bacterial Communities across Different Composite Substrates
Microbial communities play a crucial role in maintaining the health and productivity of soil ecosystems. They contribute to soil fertility, decomposing organic matter, degrading pollutants, and facilitate nutrient cycling [41]. However, continuous rose cropping can have detrimental effects on soil microbial abundance and community structure, leading to an imbalance where fungal dominance surpasses bacterial dominance [9]. To address these issues, previous studies have explored the use of microbes to improve soils affected by continuous cropping. For example, Ma et al. [42] used mycorrhizal fungi to enhance soil health and overcome obstacles in continuous upland cotton cropping. Zhang et al. [43] discovered that the immobilization of Bacillus licheniformis WL08 using tobacco stem charcoal can effectively alleviate obstacles associated with continuous pineapple cropping. These studies demonstrated the potential of microbial interventions to mitigate the negative impacts of continuous cropping and restore soil health and productivity.
Assessing the Correlation Analysis of Soil Nutrients, Soil Enzyme Activities, and Soil Bacterial Microorganisms
During vermicomposting, the introduction of substrate as a nitrogen source stimulates the growth of microorganisms, enhancing microbial activity in the soil and promoting the efficient decomposition of organic matter, which ultimately leads to an increase in soil microbial biomass flourishes. Soil microbial biomass is generally regarded as being closely linked to soil fertility [44, 45]. Comparatively, the quantity of operational taxonomic units (OTUs) for soil bacterial in groups T1, T2, and T3 surpassed that of the control (CK) group. This can be attributed to the substrate addition, introducing a significant quantity of easily accessible organic matter into the soil, and thereby stimulating the proliferation of nutrient-rich microorganisms. As a result, the abundance of OTUs increases. Evaluation of alpha diversity revealed that the incorporation of coffee grounds as a substrate exerted the most substantial influence on the prevalence of soil bacterial microorganisms.
The dominant bacterial phyla, including Proteobacteria, Bacteroidetes, and Actinobacteria, remained relatively stable across all experimental groups, indicating that the soil bacterial communities were resilient at the phylum level despite the different substrate treatments. However, through LEfSe analysis, significant differences were detected at the genus level. Specifically, we observed the upregulation of 5 genera and the downregulation of 3 genera in expression across groups. To explore the relationship between these bacterial genera and soil nutrients, correlation analysis was conducted. Results revealed strong positive correlations between substances such as available potassium, alkaline protease, cellulase, organic matter, and genera like Flavobacterium, Algoriphagus, Cellvibrio, and Pseudomonas. On the other hand, strong negative correlations were observed between these soil nutrients and genera such as Bacillus, Paracoccus and Acinetobacter. Based on these findings, we concluded that readily available potassium, alkaline protease, cellulase, and organic matter were crucial factors influencing the abundance of soil bacteria under different substrate treatments. In future studies, the potential variations and influence of selected parameters on the results will be addressed through sensitivity analyses and exploring different parameter combinations. The outcomes will contribute to improving accuracy in soil fertility assessments and enhancing our understanding of the relationship between soil bacteria and nutrient availability.
Analyzing the Factors behind Significant Differences in Bacterial Genera
The three substances used in the experiment, namely coffee grounds, camphor tree leaves, and oolong tea waste, contain significant amounts of carbohydrates (such as cellulose and lignin, etc.) and nitrogen-containing compounds (such as proteins and peptides, etc.). Cellulose, a glucose polymer, can be broken down into cellobiose and further into glucose by the action of cellulase enzymes, providing microbial organisms with a readily carbon source. One interesting observation was the increase in the genus Algoriphagus in all experimental groups, accompanied by an increase in measured cellulase content. This aligned with previous studies that have indicated that Algoriphagus has the ability to produce cellulase even at low temperatures [46]. Similarly, the genus Cellvibrio also possesses the capability to synthesize cellulase [47]. Lignin, a complex plant substance with a unique structure, is generally challenging for typical bacteria to degrade. However, the genus Flavobacterium exhibits a special metabolic pathway that can break down polycyclic aromatic hydrocarbon molecules found in lignin into smaller organic compounds. These compounds are subsequently converted into harmless substances like carbon dioxide and water [48, 49]. This metabolic pathway primarily relies on specific enzymatic substances present in Flavobacterium, such as pyrene dioxygenase and benzoate carboxylase [50].
Compared to the control group (CK), all treatment groups exhibited an increase in the relative abundance of the genus Flavobacterium, which is known for its ability to produce alkaline proteases at low temperatures [51], facilitating protein hydrolysis, thereby resulting in a rise in alkaline protease content. The genus Pseudomonas plays an important role in various metabolic processes, including amino acid metabolism, sulfide metabolism, and nitrification. It can metabolize glutamate to generate amino acids and amides, reduce sulfate to hydrogen sulfide, and participate in sulfide metabolism. Furthermore, it can oxidize nitrite and ammonia, contributing to the nitrification process in nitrogen cycling. Previous study have demonstrated that the increase in the abundance of Pseudomonas was associated with the accumulation of catechin substrates [52]. Pseudomonas acts as a catechin-degrading bacterium, converting catechins into usable carbon sources for its own growth. Additionally, Pseudomonas possesses the enzyme caffeine demethylase, enabling it to degrade caffeine [53]. The considerable presence of catechins, caffeine, and other substances in coffee grounds and oolong tea waste led to a significant increase in the abundance of Pseudomonas in treatments T1 and T3. Pseudomonas is a widely distributed plant growth-promoting rhizobacteria (PGPR) in soil [54] and is frequently used to enhance plant resistance and yield. Thus, it is reasonable to believe that this PGPR could potentially play a significant role in promoting the production of edible roses.
In this study, a significant decrease in the abundance of Bacillus, a plant growth-promoting rhizobacteria (PGPR), was observed, which aligns with the findings of Arafat et al. [52]. Furthermore, Wang et al. [55] found that Pseudomonas can utilize (-)-catechin as a carbon source and catalyze its conversion into protocatechuic acid in a laboratory setting. It is worth noting that protocatechins are known to exhibit higher toxicity to plants compared to (-)-catechins. Additionally, Pseudomonas has the ability to biotransform catechins into toxic allelopathic substances. Arafat et al. indicated that the increased concentration of these substances had no significant impact on the growth of Pseudomonas, but it significantly inhibited the growth of Bacillus. However, it is still necessary to confirm whether allelopathic substances are generated during the composting process and if the decline in Bacillus abundance is linked to compost treatment.
In comparison to the control group, the treatment group exhibited a decrease or even absence of Paracoccus and Acinetobacter, which are the main proportion of bacteria species affected. Paracoccus is a harmful species that produces nitric oxide and nitrogen dioxide, causing atmospheric damage and converting nitrates into nitrogen gas, leading to the loss of nitrogen fertilizer in agricultural soil [56, 57]. Therefore, the reduction in Paracoccus content in the experimental soil positively impacts the production of edible roses. Organic matter has been found to induce competition between plant pathogens and beneficial microorganisms, resulting in a decrease in potential infection sites for soil borne pathogens [19, 58]. This study revealed a negative correlation between organic matter and Paracoccus and Acinetobacter, suggesting that these two bacterium species might be the partial cause of continuous cropping obstacles in roses. The significant decrease in Paracoccus abundance following vermicompost treatment indicates that vermicomposting with the three substrates enhances soil conditions for the continuous cropping of roses. Similarly, the reduction in Acinetobacter population also contributes to soil improvement. Acinetobacter, which belongs to the Proteobacteria group, can act as opportunistic pathogens. Maintaining a high abundance of Acinetobacter in the soil can have long-term detrimental impacts on soil ecosystems. After the composting process, beneficial microorganisms in the soil increase in number, competing with and suppressing the growth of pathogenic bacteria through nutrient and niche competition [59, 60]. Hence, the extinction of this species can enhance the safety of the facility’s environment by reducing the prevalence of soil-borne diseases.
The relative abundances of the genera Flavobacterium, Algoriphagus, Cellvibrio, Pseudomonas, and Glutamicibacter exhibited an overall increase in all treatment groups. However, when compared to the control group (CK), T1 and T3 exhibited distinct dominant genera. In T1, the dominant genera was Cellvibrio, whereas in T3, it was Flavobacterium. . This disparity in dominance can be attributed to the higher concentration of active compounds (such as tea polyphenols, caffeine, organic acids, etc.) found in coffee grounds and oolong tea waste extract in comparison to camphor tree leaves [4, 5]. These compounds likely have direct or indirect impact on the metabolism, growth, and composition of bacteria communities. Additionally, we also noticed a significant rise in the abundance of Bergeyella in T3. Due to the scarcity of research on the presence of Bergeyella in soil, the consequences of its increased abundance on the soil remain uncertain.
Conclusions
There have been numerous studies on the use of compost products to overcome continuous cropping challenges in crops. However, little research has been conducted on the utilization of earthworm compost products in alleviating continuous cropping issues in rose cultivation soil. Hence, this study aimed to examine the effects of vermicomposting using different substrates on soil chemical properties, enzymatic activity, and bacterial communities. The results indicated that all three substrates contributed to improved soil nutrient content and enhanced the activity of certain enzymes to varying degrees. Notably, the addition of oolong tea waste demonstrated the most significant improvement in soil chemical properties. Furthermore, the use of these substrates resulted in alterations to the bacterial community structure in the soil. Although the dominant bacterial genera differed among the substrates, there was an overall increase in beneficial bacterial genera associated with enhancing soil fertility, while detrimental bacterial genera experienced a decrease. The specific mechanism through which coffee grounds and oolong tea waste affect bacterial communities require further investigation. By effectively utilizing organic waste resources and minimizing wastage, we can achieve resource reuse and reduce the environmental burden posed by waste. It is important to note that different substrates may have varying effects on soil improvement depending on the specific circumstances. This study focused solely on continuous rose cultivation in soil, but future research could explore different soil types to gain a broader understanding of the subject matter.

