

Introduction
Chinese hickory (Carya cathayensis Sarg.) belongs to Juglandaceae family. It is a unique, woody nut and oil tree species. Its natural distribution area is confined in limestone mountain regions in Zhejiang and Anhui Provinces of China. The popularity and demand for Chinese hickory have been increasing due to the nut fruits’ tastes and health benefits [1]. In the initial stage, farmers brought double benefits of Chinese hickory yield and quality through large-scale application of chemical fertilizer. However, overtime, the consequence of large-scale application of chemical fertilizer is that the soil acidification is becoming more and more serious, which may cause Chinese hickory to suffer from aluminum (Al) toxicity. Long-term application of excessive chemical fertilizer leads to early senescence and even death of Chinese hickory plants and exposure to various diseases and pests, especially the canker and root-rot diseases of Chinese hickory [2], which causes serious damage to the forest and consequently reduces the yield of Chinese hickory.
Soil acidification can negatively impact the sustainability of crop production systems. Studies have shown that long-term application of nitrogen fertilizer can reduce soil pH [3]. Al is the main stress factor limiting crops productivity on acid soil. The earth soils contain abundant Al in the form of silicates, oxides and hydroxides. However, most Al in soils are nontoxic to living organisms due to their inactivity [4]. The soil acidity is mainly controlled by labile Al. The hydrolysis of Al3+ produces a moderately acidic environment, so many properties of acidic soils are controlled by the chemical properties of Al [5]. As soil pH decreases (pH≤ 5.5), Al is converted to toxic Al3+, and it is readily absorbed and interferes with normal growth of plants [6]. Al exposure leads to increased reactive oxygen species (ROS) in cells, lipid peroxidation, organelle dysfunction and damage, and inhibition of cell elongation and division [7]. When the pH is lower than 4.0, tea plant growth is inhibited, affecting both the quality and quantity of tea production, and jeopardizing human health [8]. Therefore, long term application of nitrogen fertilizer may lead to aluminum toxicity stress on plants, changes in metabolites and deteriorating crop growth.
It is considerable interest in mechanisms of plant Al resistance exhibited by researchers around the world. Some plants chelate Al by releasing organic acid anions (OAA),such as malate, citrate, oxalate [6, 9]. Winkel Shirley found that in addition to OAA, antioxidant compounds such as phenolics also have the capacity to chelate toxic metal ions due to their functional groups hydroxyl (-OH) and carboxylic (-COOH), reducing the harmful effects of Al on plants [10].
Metabonomics is a science that studies biological systems by investigating the changes of metabolites or their changes over time after stimulation or disturbance of biological systems, including cells, tissues or organisms. Metabolomic approaches are an indirect way to evaluate changes in gene or protein expression resulting from environmental stresses and can provide information on tolerance mechanisms. Metabolomic approaches are increasingly used to study abiotic stresses. Toma´s Grevenstuk finds that the internal detoxification of Al in plantago almogravensis plantlets is associated with accelerated consumption of carbohydrate resources.[11] Al toxicity could be mitigated with boron by altering the metabolic patterns of amino acids and carbohydrates rather than organic acids in trifoliate orange [12]. Metabonomic methods can help us better understand Al resistance mechanism of crops. Studies have shown that excessive application of nitrogen fertilizer is one of the key important reasons for the degradation of Chinese hickory forest [13], but the physiological and biochemical mechanisms of soil acidification limiting the growth of Chinese hickory have not been reported yet.
Therefore, using the effects of acid stress caused by excessive nitrogen fertilizer and direct Al stress on the nutrition of Chinese hickory, combined with the metabonomic study, this paper analyzes the changes of metabolites in Chinese hickory leaves under excessive nitrogen fertilizer and direct Al stress, and aims to reveal the response mechanism and resistance changes of Chinese hickory under excessive nitrogen fertilizer. The results can provide guidance for optimal management of Chinese hickory forest.
Materials and Methods
Overview of the Experimental Area
The experimental Chinese hickory forest land was located in Baijiang Town, Tonglu County, Hangzhou City, Zhejiang Province (29º49’20.40’’N, 119º14’50.85’’E). The applied nitrogen fertilizer is urea and Aluminum is aluminum sulfate reagent (Al2(SO4)3·18H2O (AR), (Sinopharm Chemical Reagent Co., Ltd). The soil of experimental area belongs to red soil, and the tree age is 15 years old. The basic chemical properties of the soil in the pecan forest land of the test site are as follows:pH 5.28, alkaline hydrolyzable nitrogen 155.46 mg/kg, available phosphorus 27.44 mg/kg, available potassium 66.92 mg/kg, organic matter 10.50 g/kg.
Experimental Design
The field experiment was conducted with 3 treatments. The applied materials and dosage were as follows: Treatment 1 (CK), no materials addition; Treatment 2 (N), urea, 0.3 kg/plant; Treatment 3 (Al), Al2(SO4)3·18H2O, 0.5 kg/plant. Each treatment was replicated four times. The materials were applied in March 2018.
The plant samples were collected in October 2018. Fresh leaf samples were transported from the field over dry ice and then frozen immediately in liquid nitrogen upon arrival in the laboratory and stored at −80ºC. The samples were divided into two portions, one of which was dried to constant weight in an oven at 70ºC and was milled for chemical analysis. The other samples, for metabolomics analysis, were stored at −80ºC immediately until use.
Analytical Measurement
Plant elemental determination: The concentrations of elements in plant samples were determined after digestion with concentrated sulfuric acid-hydrogen peroxide. The N, P, and K were measured by indophenol blue spectrophotometry, molybdenum blue colorimetry, and flame photometry, respectively. Trace elements were determined with inductively coupled plasma optical emission spectrometry (Optima 7000 ICP-OES).
Metabolomics analysis: For the extractions, 50 mg of fresh leaf material were ground in liquid nitrogen with a mortar and pestle with 800 μL methanol: water (80:20). The microcentrifuge tubes were vortexed at 120000 rpm for 15 min (4ºC) and then sonicated in a 25ºC water bath for 30 min. All the supernatant was transferred into a centrifuge tube and stand at −40ºC for 1h and then vortexed at 120000 rpm for 15 min (4ºC). The supernatant (200 μL) was used for LC-MS analysis.
Analysis platform: LC-MS (Waters, UPLC; Thermo, Q Exactive). ACQUITY UPLC HSS T3 (2.1 mm × 100 mm, 1.8 µm) column was used for chromatographic separation of all analytes. The column was maintained at 40ºC throughout the run. A dual eluent mobile phase comprised of water with 0.1% formic acid and acetonitrile at 300 µL/min was used for separation. The gradient of the mobile phase is shown in Table 1.
Parameters of positive mode and negative mode (simultaneous operation) of electric spray (ESI) are as follows:
ESI+: Heater Temp 300ºC; Sheath Gas Flow rate, 45 arb; Aux Gas Flow Rate, 15 arb; Sweep Gas Flow Rate, 1 arb; spray voltage, 3.0 KV; Capillary Temp, 350ºC; S-Lens RF Level, 30%.
ESI-: Heater Temp 300ºC, Sheath Gas Flow rate, 45 arb; Aux Gas Flow Rate, 15 arb; Sweep Gas Flow Rate, 1 arb; spray voltage, 3.2 KV; Capillary Temp, 350ºC; S-Lens RF Level, 60%.
Statistical Analysis
E1: The data were processed by Microsoft Office Excel 2010. The statistical analyses were run by ORIGIN 11.0 and SPASS 22.0. Duncan’s new complex range method (p<0.05) was used for significant comparison.
E2: In order to better explore the reaction mechanism of Chinese hickory under soil acidification and the effect on its resistance, the following comparison was set: CK vs N and CK vs Al.
The Compound Discoverer3.1 (CD) software was used for mass spectrometry and database search. Then, SIMCA software (V14.1, Umetrics AB, Umea, Sweden) was used for multivariable. statistics. Model construction analysis included principal component analysis (PCA) and orthogonal projection to latent structures discriminant analysis (OPLS-DA). The differential metabolites were screened by the combination of student t-test (Get P-value) and Variable Importance in the Projection (VIP) of orthogonal partial least square method. Analysis of differential metabolites includes Hierarchical Clustering Analysis and Pathway Analysis.
Results
Effects of Different Treatments on Nutrient Uptake in Plant Leaves
The nutrients of N, P and K are three key elements for plant growth and yield production. Table 2 indicated that there was a significant difference between the treatments for N and K concentrations in the leaves. Compared with CK, leaf N concentrations in plant treated with urea significantly increased by 35.9% but decreased by 27.4% under Al treatment. By contrast, leaf K concentrations significantly decreased (p<0.05) by 22.4% (N treatment) and 11.2% (Al treatment) compared with CK, respectively. For leaf P, there was no significant difference among different treatments. The other essential elements are also vital for plant survival and they play their respective roles in the process of plant metabolism, controlling and maintaining the complex life activities of plants. The concentrations of Ca and Mg in T2 and T3 treatments were decreased (compared with CK) by 13.4, 16.9% and 30.2, 7.1%, respectively. Moreover, the concentrations of B in Chinese hickory leaves decreased significantly, and T3 had a greater impact on leaf B than T2 . In contrast, the concentrations of Cu and Zn in Chinese hickory leaves all decreased though after N application treatment as well as Al application treatment but there was no significant difference among different treatments (Table 2).
Table 2.
Effects of different treatments on concentrations of N, P, K, Ca, Mg, Cu, B, Zn in leaves of Chinese hickory.
| N | P | K | Ca | Mg | Cu | B | Zn | |
|---|---|---|---|---|---|---|---|---|
| mg/g | mg/g | mg/g | mg/g | mg/g | mg/kg | mg/kg | mg/kg | |
| T1 (CK) | 14.33b | 2.87a | 16.29a | 20.68a | 4.11a | 23.0a | 24.3a | 174.5a |
| T2 (N) | 19.99a | 2.54a | 12.64c | 17.91b | 2.87b | 20.9a | 21.7b | 169.3a |
| T3 (Al) | 10.41c | 2.78a | 14.47b | 17.18b | 3.82a | 18.9a | 18.3c | 171.9a |
Table 3.
LC-MS identification results in positive and negative mode.
| Compounds | Amino acids | Nucleotides | Carbohydrates | Organic acids | Falvonoids and their glycosides | Plant growth regulations | Alkaloids | Other compounds | Total |
|---|---|---|---|---|---|---|---|---|---|
| ESI+ | 18 | 9 | 11 | 75 | 45 | 4 | 7 | 76 | 245 |
| ESI- | 11 | 5 | 15 | 70 | 61 | 4 | 0 | 14 | 180 |
In summary, except for N concentrations in plant leaves, the application of nitrogen fertilizer, similar to Al stress, would inhibit the uptake of soil nutrients by Chinese hickory, especially Ca, Mg and B were more profoundly affected.
Metabolomics
LC-MS Identification Results
To study the change patterns of Chinese hickory metabolomics under soil acidification, the non-targeted LC-MS method was used for metabolic analysis. ESI+ identified 245 metabolites and ESI- identified 180 metabolites (Table 3).
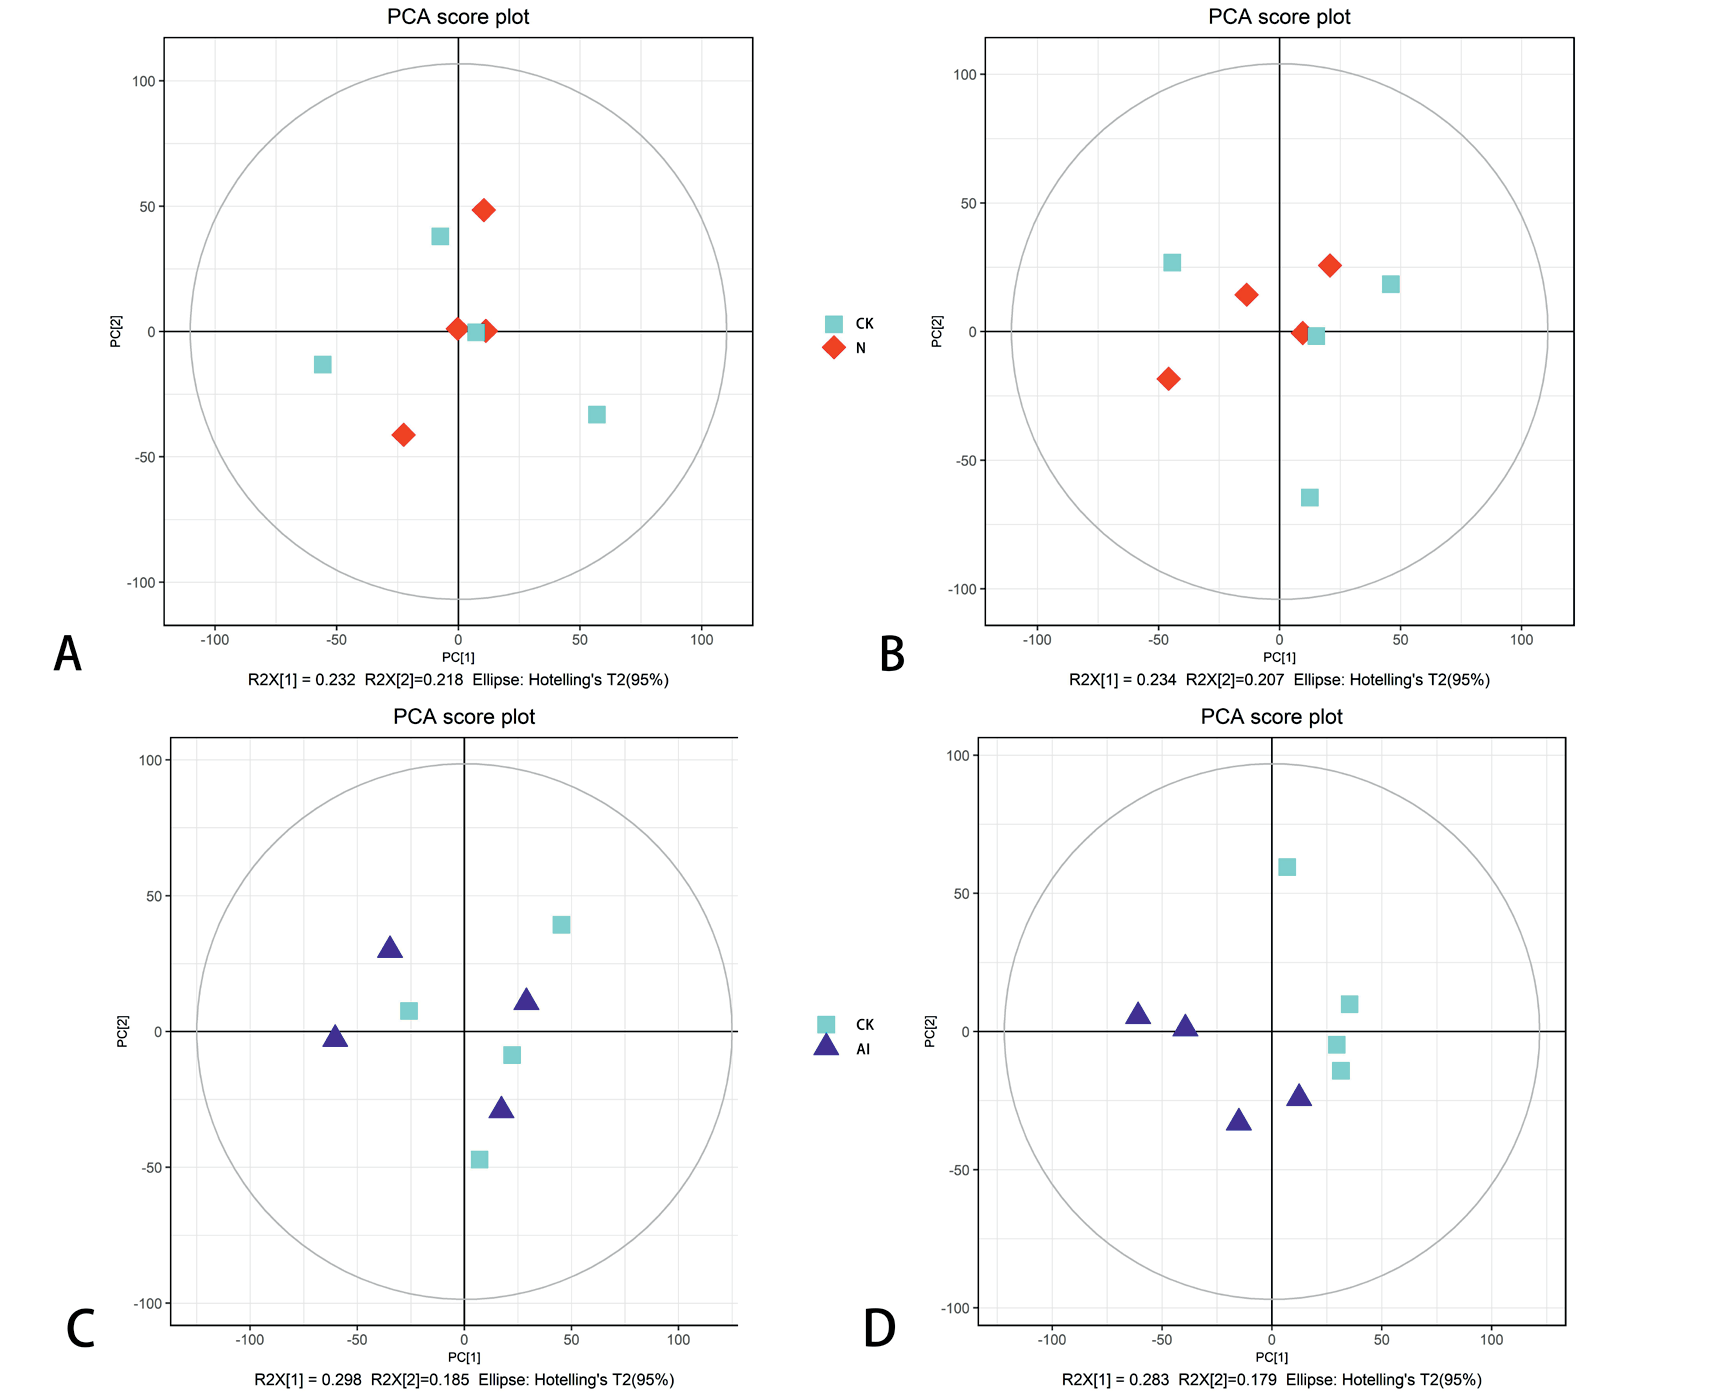
Principal Component Analysis (PCA) and Orthogonal Projection to Latent Structures Discriminant Analysis (OPLS-DA)
Firstly, according to CK vs N and CK vs Al (in the anionic mode and the cationic mode), the PCA model that fit the four principal components was obtained using principal component analysis (Fig. 1). In the anionic mode, CK vs N accounted for a variance of 23.2% by PC1 and 21.8% by PC2, and 23.4% by PC1 and 20.7% by PC2 in the cationic mode. In the anionic mode, CK vs Al accounted for a variance of 29.8% by PC1 and 18.5% by PC2, and 28.3% by PC1 and 17.9% by PC2 in the cationic mode. All Chinese hickory leaf samples are within hotelling’s t-squared ellipse. But it can be seen from the figure that the samples between treatments have the phenomenon of regional intersection (No obvious separation), regardless of CK vs N or CK vs Al. The disadvantage of PCA is that it cannot ignore the intra-group error and eliminate the random error irrelevant to the research purpose, so it is an unsupervised analysis method. So it is not conducive to the discovery of intergroup differences and differential compounds, and the supervised OPLS-DA model was used for further analysis. As shown in the OPLS-DA chart (Fig. 2), we can filter out the orthogonal variables in the metabolites that are not related to the classification variables, and analyze the non-orthogonal variables and orthogonal variables respectively, to obtain more reliable information about the correlation between the inter-group differences of the metabolites and the experimental group. As shown in the OPLS-DAchart, the samples of CK were mainly distributed on the left side of the confidence interval, and the samples of experimental group are mainly located on the right side of the confidence interval, which indicates that the model can effectively distinguish the samples. The samples of the experimental group and the control group can be clearly distinguished in the first principal component according to OPLS-DA analysis, indicating that there are differences in metabolites between the experimental groups (N and Al treatments) and the control group (CK).
Differential Metabolite Analysis
To classify the metabolites with the same metabolic characteristics into one group and the change characteristics of modern metabolites in the experimental group, we carried out a hierarchical clustering analysis of the different metabolites.
Fig. 2.
OPLS-DA score plots of different samples. a) OPLS-DA score plots of CK vs N in anionic mode (ESI-); b) OPLS-DA score plots of CK vs N in cationic mode (ESI+); c) OPLS-DA score plots of CK vs Al in anionic mode (ESI-). d) OPLS-DA score plots of CK vs Al in cationic mode (ESI+).
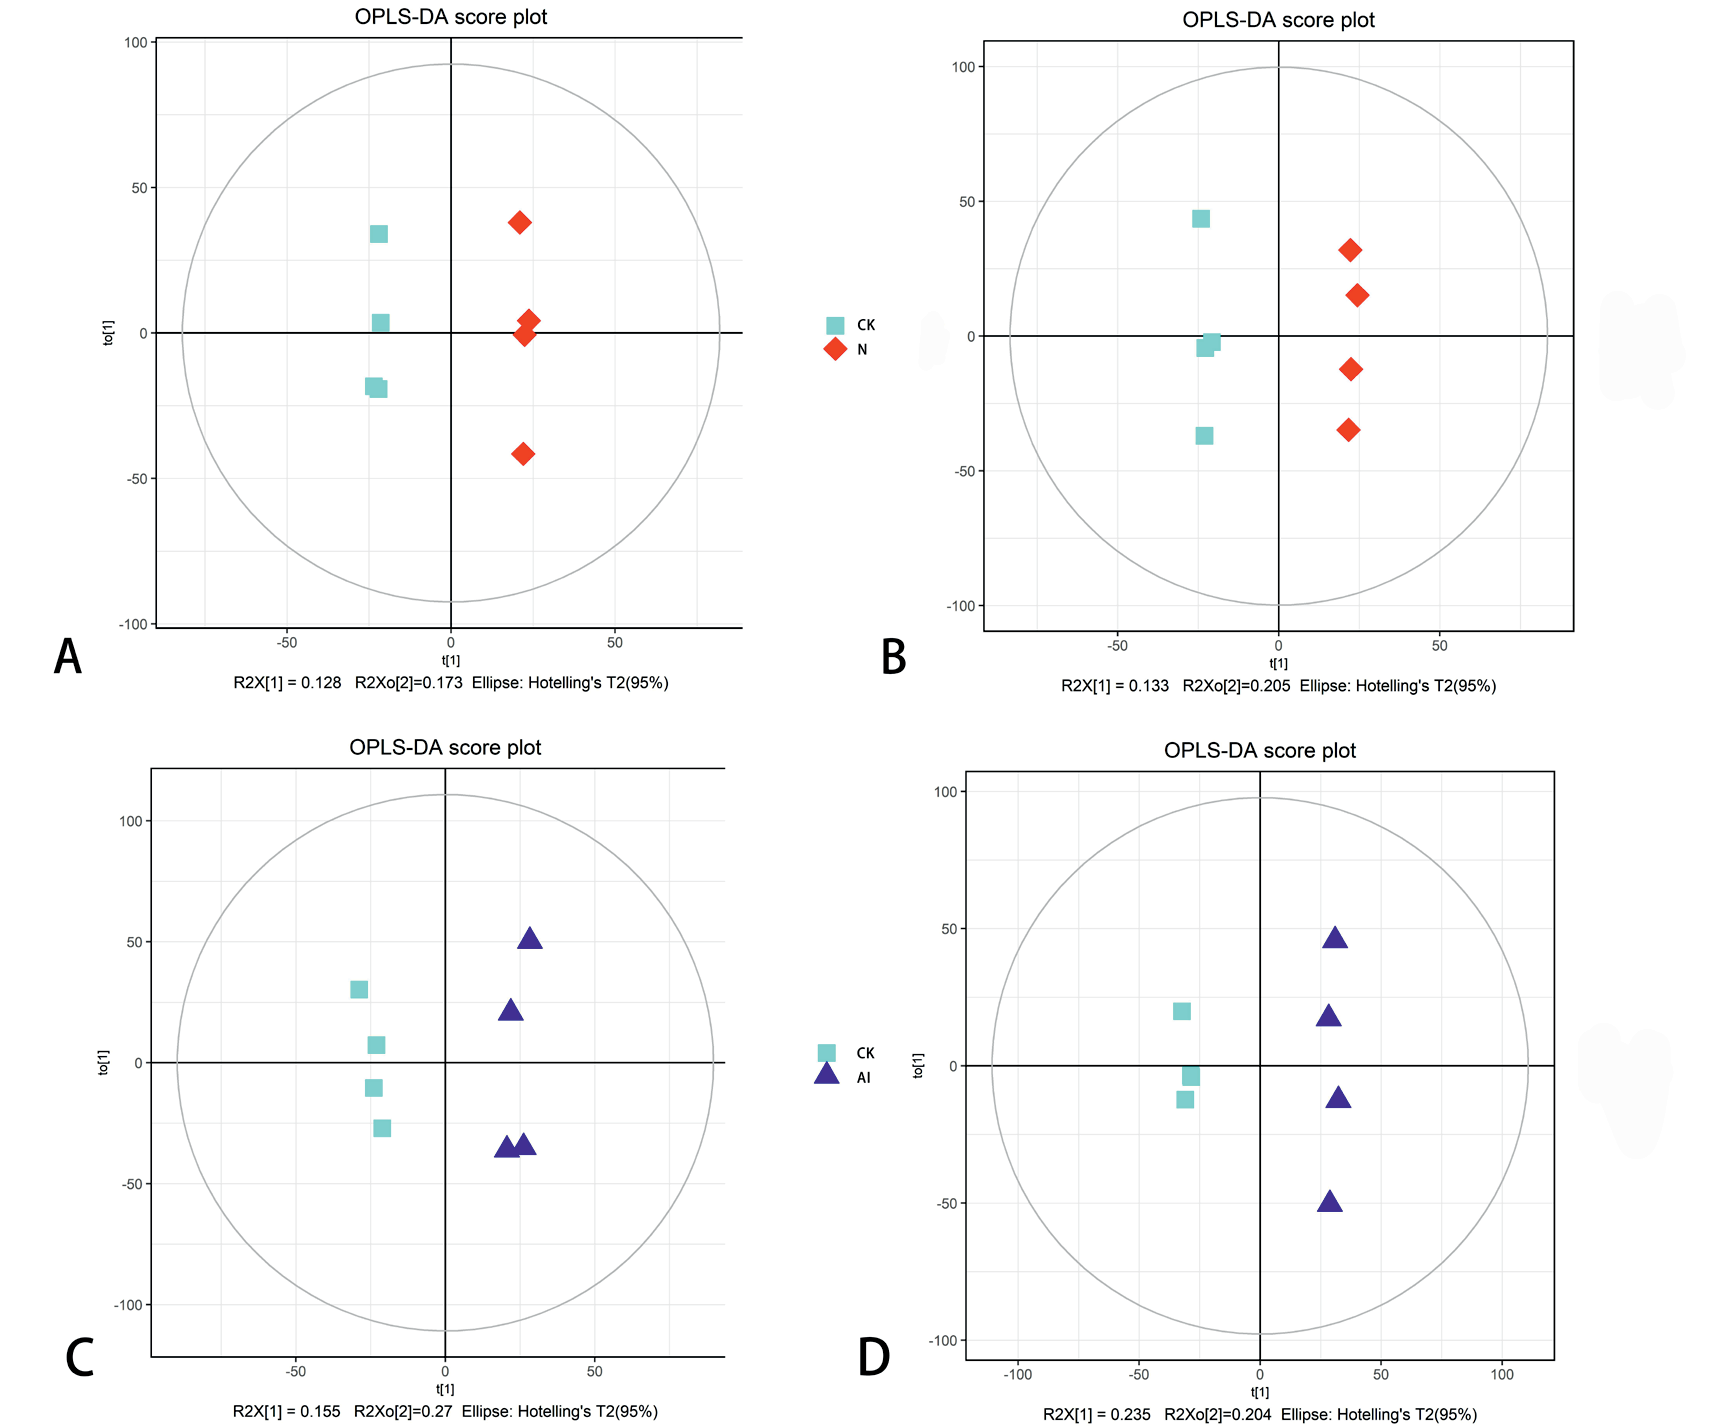
Fig. 3.
Hierarchical cluster analysis of differential metabolites in Chinese hickory leaves. a) CK vs N (ESI-); b) CK vs N (ESI+); c) CK vs Al (ESI-); d) CK vs Al. (ESI+). The abscissa in the Fig. represents different treatments, the ordinate represents the different metabolites compared in this group, and the color blocks at different positions represent the relative expression of metabolites at corresponding positions. The screening criteria for differential metabolites used were: the P-value of the student's t-test is less than 0.05 (P<0.05), and the VIP of the first principal component of the OPLS-DA model is greater than 1 (VIP>1).
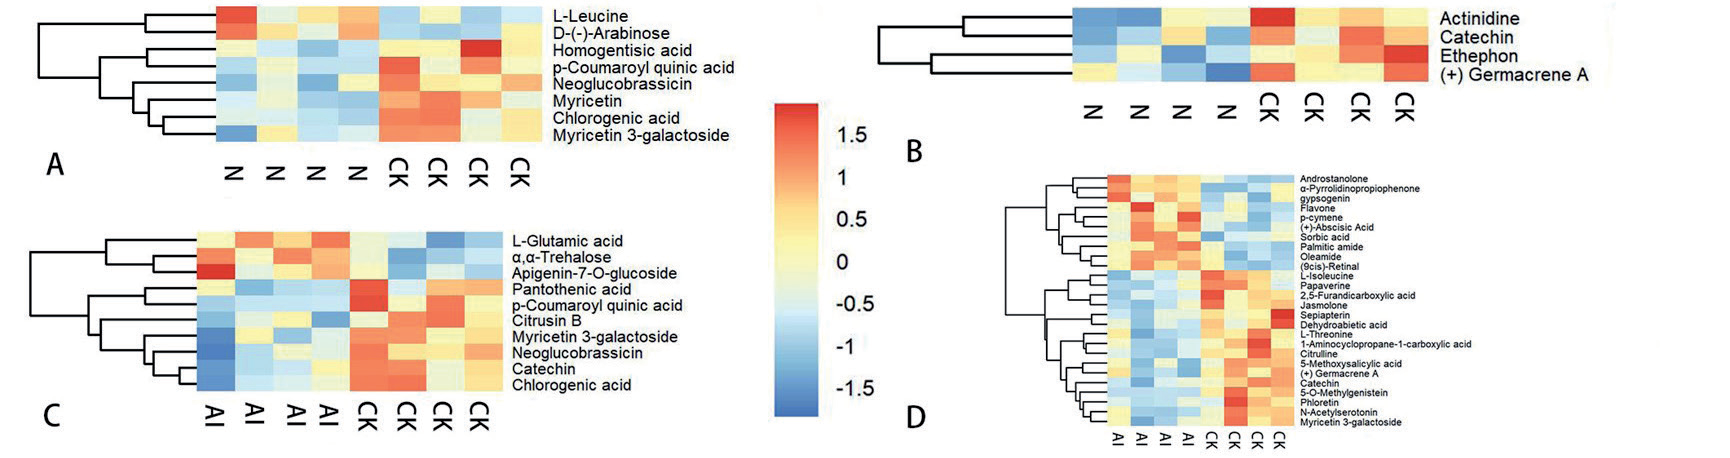
Compared with T1, T2 and T3 metabolites changed to a certain extent. As shown in Fig. 3, compared with the CK, the content of 10 metabolites in T2 decreased significantly (p-coumaroyl quinic acid, chlorogenic acid, (+) cermacrene A, catechin, myricetin, homogentisic acid, myricetin 3-galactoside, actinidine, neoglucobrassicin, ethephon) and the content of 2 metabolites increased significantly (L-Leucine, D-(-)-Arabinose). Compared with T1, there are 23 metabolites whose relative content of T3 is downregulated, among which the top 10 metabolites with downregulated differential multiple are 5-o-methylgenistein, p-coumaroyl quinic acid, papaverine, phloretin, (+) germacrene A, N-acetylserotonin, chlorogenic acid, catechin, myricetin, myricetin 3-galactoside, and citrulline. There are 13 metabolites with upregulated relative content. The metabolites with the top 10 difference multiples were flavone, palmitic amide, (+)-abscisic acid, p-cymene, α-pyrrolidinopropiophenone, androstanolone, α, α-trehalose, oleamide, (9cis)-retinal, apigenin-7-o-glucoside. Through comparison, it was found that the contents of metabolites between CK vs N and CK vs Al have similar parts, including p-coumaroyl quinic acid, chlorogenic acid, catechin, (+) germacrene A, myricetin 3-galactoside and neoglucobrassicin. We speculate that these metabolites may be the main regulators of Chinese hickory to soil acidification stress, or related to the effect of soil acidification on Chinese hickory resistance.
Metabolic Pathway Analysis
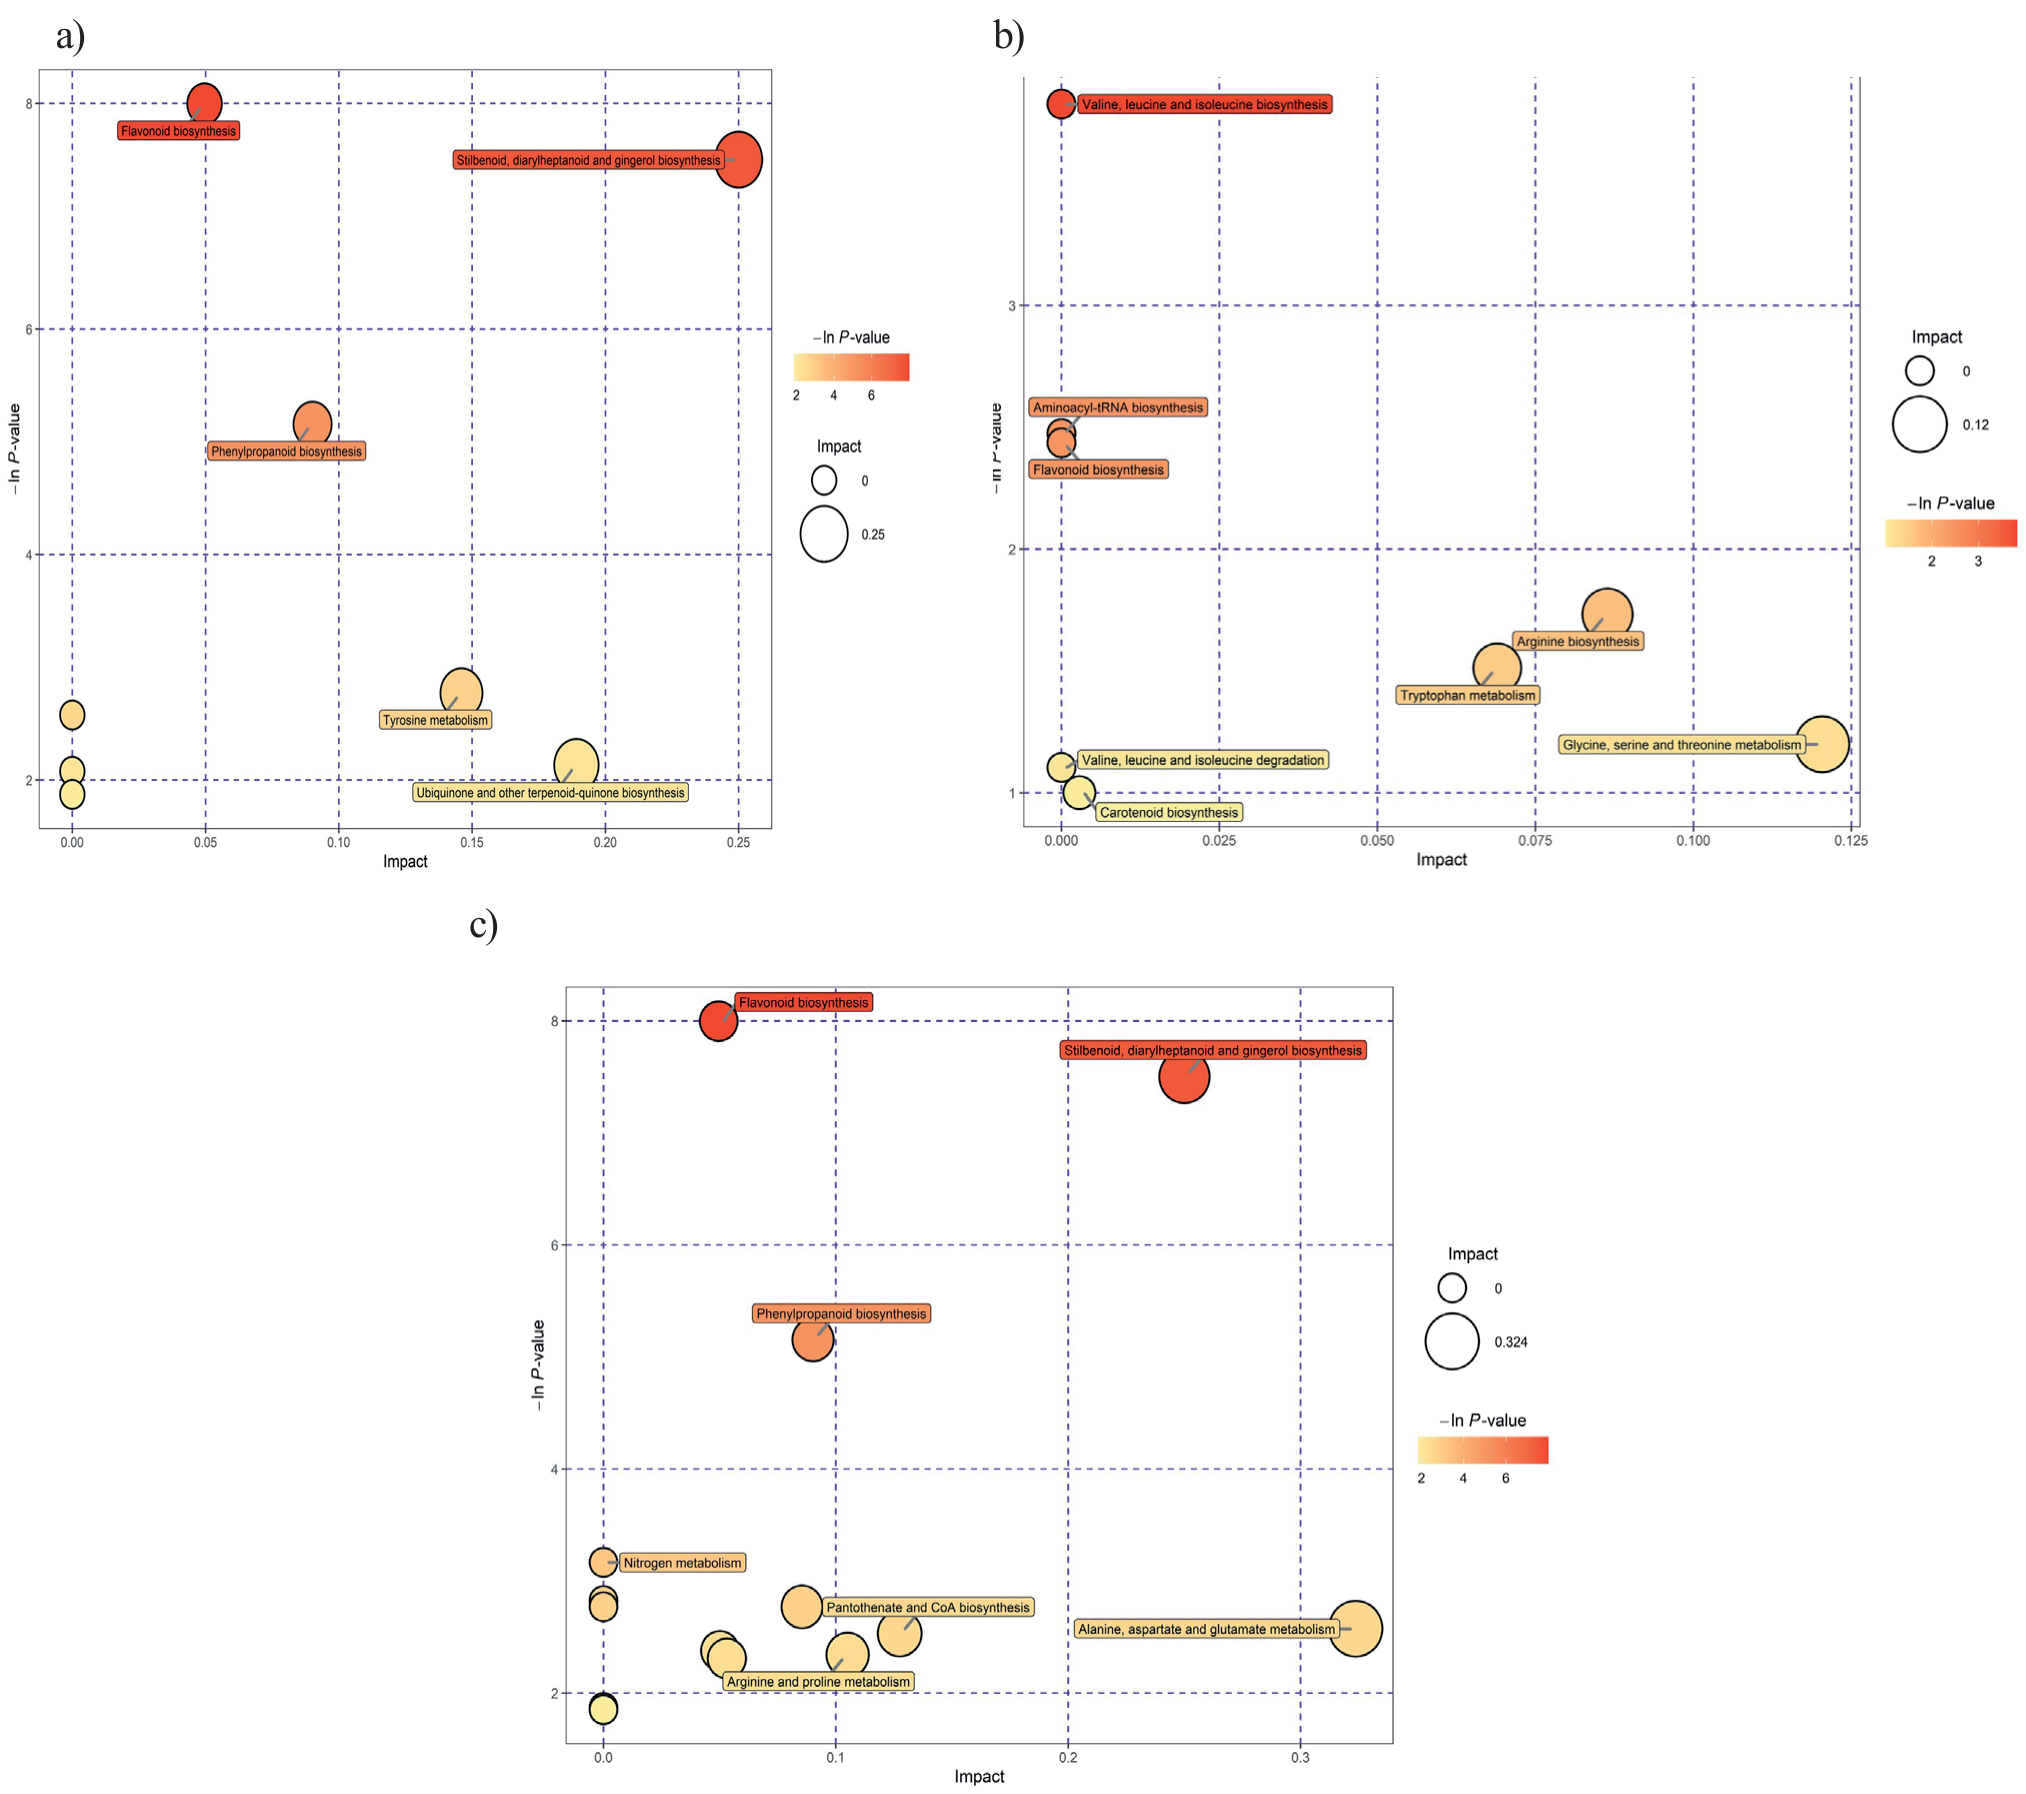
Using KEGG database to annotate the differential metabolites, and then comprehensively analyze the pathways of differential metabolites (including enrichment analysis and topology analysis), we can further screen the pathways and the pathway with the highest correlation with the difference of metabolites is obtained. KEGG topology analysis was performed on the metabolic pathways of differential metabolite enrichment, and the results are shown in the bubble diagram below (Fig. 4).
The differential substances in CK vs N were annotated into 9 metabolic pathways, of which 5 metabolic pathways changed significantly. The differential substances in CK vs Al were annotated into 22 metabolic pathways, of which 15 metabolic pathways changed significantly. We found that Flavonoid biosynthesis, Phenylpropanoid biosynthesis, Tyrosine metabolism, Stilbenoid, diarytheptanoid, and gingerol biosynthesis were annotated at the same time.
Discussion
When the environment changes, it will have varying degrees of impact on the metabolites in the plant body, and nutrient elements (such as N, P, K, Ca, Mg, Cu, B, Zn) are important components of the metabolites. Explore the physiological processes of Chinese hickory plants under aluminum stress by combining the changes in metabolites and nutrient elements in leaves.
N, P, and K play key important roles in plant life activities. The N is an important component of macromolecules such as proteins, nucleic acids, and chlorophyll. In all organisms, protein is the most important, because it is at the center of metabolic activities. The application of nitrogen fertilizer significantly increased the concentrations of N in Chinese hickory leaves, and the results were consistent with the findings of Lincoln Zotarelli [14]. He pointed out that the application of nitrogen fertilizer can significantly increase the concentrations of N in plants. The high content of soil active Al may inhibit the activities of rhizosphere nitrogen fixation microflora and soil enzymes, which reduce the supply of soil available N, and gradually reduce the total N in plants [15]. K can improve product quality and adapt to the adverse external environment. The significant decrease of leaf K concentrations in T2 and T3 implied that the stress resistance of Chinese hickory plant decreased.
The results showed that both the application of N and Al inhibited the absorption and transport of some nutrient elements (P, K, Ca, Mg, Cu, B, Zn) to varying degrees.There is a certain synchronicity between the effects of N treatment and Al treatment on the nutrient elements in the leaves of Chinese hickory. Al toxicity causes root injury and therefore results in inhibition of root nutrient uptake and transport to the above-ground plant parts [6, 8, 16]. The present experimental results indicate soil Al toxicity is the main factor of Chinese hickory forest degradation caused by long-term application of nitrogen fertilize, which is consistent with previous studies [17, 18]. It is speculated that part of the reason is that different forms of active Al dissolved from acidic soil block the cation channel. The lower Ca and Mg concentrations in plant tissues in the presence of Al were due to the fact that the two ions compete for binding to Al and participate in the ion channel active sites during absorption [19, 20].
Fig. 4.
KEGG topology analysis of bubble graphs: Each bubble represents a KEGG pathway; the horizontal axis represents the relative importance impact value of metabolites in the pathway; the vertical axis represents the enrichment significance of the metabolite pathway -ln (P-value). The size of the bubbles in the Fig. represents the impact value. The larger the bubble, the greater the importance of the pathway, which is the basis for screening metabolic pathways. a) KEGG topology analysis of bubble graphs of CK vs N. (There is no metabolic pathway which have significant change in positive mode (ESI+).); b) KEGG topology analysis of bubble graphs of CK vs Al (ESI-); c) KEGG topology analysis of bubble graphs of CK vs Al (ESI+).
Although the concentrations of trace elements in plants are very low, they are activators of physiological processes and important components of many enzymes. They play a vital role in the life activities of plants and the change in their concentrations will also lead to the change in plant metabolic activities and resistance. Cu plays an important role in plant growth and stress resistance. Cu is a component of certain oxidases (such as ascorbic acid oxidase, reactive oxygen species, etc) that can affect the redox process [21, 22]. Ascorbate peroxidase and the glutathione cycle (AsA-GSH cycle) respond to control ROS levels at the physiological level [23]. There are many kinds of enzymes in plants. Under the synergistic action of some enzymes, they can prevent oxygen poisoning in plants, effectively protect cells and the body itself, and enhance the tolerance of plants under adverse stress. The main function of Mg is as the central atom of chlorophyll a and chlorophyll b porphyrin ring, which plays an important role in chlorophyll synthesis and photosynthesis. Studies have shown that Al stress can reduce the photosynthetic and antioxidant capacity of plants [10, 24]. B is involved in carbohydrate metabolism. And B deficiency significantly increased the synthesis of abscisic acid (ABA) in plants [25]. Among the different metabolites of Al treatment, the significant upregulation of abscisic acid is the stress response of Chinese hickory to Al stress. After Al stress, the decrease of these elements concentrations in plant leaves indicated that the resistance of Chinese hickory was weakened.
The most important response of plants to stress is the change of metabolism, that is plants induce a series of special metabolites by regulating the metabolic network, so as to achieve the defense effect against biological and abiotic stress. Metabonomics can reveal the response mechanism of plants under stress by monitoring the changes of metabolites of the plant system under stress or stimulation. It is a good way to study plant stress resistance. In the present experiment, there were 36 significantly different metabolites in CK vs Al, 24 more than CK vs N. This showed that the response of Chinese hickory leaves to Al treatment (T3) stress was more intense than that of T2 treatment. We speculate that there are two reasons: the active Al in T2 soil does not reach the level in T3; effects of exogenous N on Chinese hickory.
Metabonomics data show that there are many similarities in metabolites and metabolic pathways between CK vs N and CK vs Al, indicating that the effect of soil acidification on Chinese hickory is mainly Al toxicity. Both flavonoid biosynthesis and phenylpropanoid biosynthesis of KEGG metabolic pathway are annotated. Flavonoid metabolism is an important branch of phenylpropanoid metabolism and gives rise to the largest class of polyphenolic metabolites, approximated to encompass more than 6,000 compounds [26]. P-coumaroyl quinic acid, chlorogenic acid (CGA), and catechin are important disease-resistant substances or intermediates in flavonoid biosynthesis and phenylpropanoid biosynthesis [27-29]. Hydroxy cinnamoyl-CoA quinate hydroxycinnamoyl transferase can catalyze coffee and quinine acid coenzyme A to generate chlorogenic acid [30]. During their evolution, plants acquired the ability to synthesize different phenylpropanoid compounds like chlorogenic acid, which plays a vital role in resistance mechanisms to abiotic stresses [27, 31]. In the process of long-term evolution, plants have developed a variety of adaptive strategies to deal with Al toxicity, among which internal tolerance and external exclusion are widely considered the main strategies. In recent years, a large number of studies have found that phenols play an important role in the mechanism of Al tolerance in plants [10]. Haruma Toshikatsu’s study found that miscanthus can detoxify Al by producing CGA and localizing Al in cell walls [32, 33]. The biosynthesis of catechin is a tributary of flavonoid metabolism [27]. It was found that maize roots exposed to Al secreted a large number of phenolic compounds (including catechin), indicating that their ability to chelate metals can be used as an in vivo mechanism to improve Al toxicity. Al-catechin complexes were formed when tea is under Al stress [34]. Under the condition of long-term application of nitrogen fertilizer, the metabolites (such as CGA and catechin) in Chinese hickory decreased significantly, which may be that these metabolites are involved in the physiological process of combating Al toxicity.
CGA and catechin are naturally-occurring plant defense metabolites. CGA and catechin have been proven to promote plant health, antibacterial and antiviral properties in many studies [28, 30]. Because of their excellent antibacterial and disease resistance potential, CGA and catechin are also widely used in modern medicine and have a great impact on human health [35]. The content of CGA in the chrysanthemum is inversely proportional to the amount of nitrogen fertilizer. With the increase in nitrogen fertilizer, the activity of phenylalanine ammonia-lyase (PAL) which is a key enzyme in the phenylpropanoid biosynthesis pathway decreased significantly [36, 37]. Therefore, CGA and catechin may be important disease-resistant substances to prevent canker disease and root-rot disease. Long-term application of nitrogen fertilizer makes CGA and catechin in Chinese hickory used to fight Al toxicity. The significant decrease in CGA and catechin may be the main reason for the increased risk of Chinese hickory. What’s more, Chinese hickory are famous for their rich nutritional value. Flavonoids, stilbenoid, diarylheptanoid, and gingerols have good health care functions [38-40]. The metabolic pathways of these compounds changed significantly in the experiment, indicating that soil acidification may also affect the quality of Chinese hickory.
At present, people generally use quicklime to improve the soil acidification of Chinese hickory forest. However, long-term application of quicklime will cause adverse conditions such as soil hardening and soil nutrient decline. Studies have also shown that polyphenols (such as CGA, catechin, etc) provide tolerance to the plant against various stresses by exogenous application [41-43]. CGA and catechin may be more environmentally friendly and safer for biological use. The effects of exogenous phenols such as CGA and catechin on Al tolerance and plant diseases and insect pests of Chinese hickory can be used as the next research direction.
In summary, the long-term application of nitrogen fertilizer results in Chinese hickory being subjected to aluminum toxicity stress, which in turn causes changes in the content of nutrients and metabolites in the plant body. And these changes are all a comprehensive responses of Chinese hickory plant to soil aluminum toxicity.
Conclusions
The present experiment confirmed that Chinese hickory is an acid-sensitive plant species and Al could be the key toxic factor in acid soils that resulted in the degradation of Chinese hickory forest. Through metabolomics study, it was found that a variety of metabolites in Chinese hickory leaves changed when Chinese hickory reacted to soil acidification. Among them, phenolic substances (such as CGA and catechin) may be involved in the regulation of Chinese hickory against Al toxicity. Long-term application of nitrogen fertilizer resulted in decrease of CGA and catechin in Chinese hickory. The significant decrease in CGA and catechin may be the main reason for the increased risk of Chinese hickory growth and production. This study provides a basis for future studies on improving degraded Chinese hickory forest and curing canker disease and root-rot disease of Chinese hickory, and is of great theoretical reference importance.

