

Introduction
Plants can change the physicochemical properties and microbial community structure of soil via root exudates and litter, thus affecting subsequent plant growth and altering the competitive relationships of coexisting plants and community structure, which is called soil legacy effects [1]. Soil legacy effects on subsequent plants may be negative, positive, or neutral. In agricultural production, creating positive soil legacies through innovative agricultural management can enhance agricultural productivity and achieve agricultural sustainability [2]. Inoculation with arbuscular mycorrhizal fungi (AMF) is one of the soil management practices that can improve positive soil legacies. AMF can improve soil structure, increase plant nutrient uptake, and enhance plant stress resistance via extensive mycelial networks [3]. Therefore, AMF are widely used in agricultural production as a new type of biological fertilizer [4].
Nowadays, the rate of global warming over the last 50 years is unprecedented, and if the warming exceeds 1.5ºC in the short term, terrestrial ecosystems will face serious threats [5]. The effects of warming on AMF are complex, including direct effects on the diversity and function of AMF and indirect effects on the symbiotic relationship between plants and AMF [6]. On the one hand, elevated temperatures below optimal levels can promote fine root growth and the production of root exudates [7], thus enhancing mycorrhizal effects. On the other hand, warming can inhibit mycorrhizal effects due to water deficit [8] or eliminate the buffering effect of AMF on nutrient leaching due to lower mycorrhizal colonization [9]. AMF are more tolerant to increases in temperature than other microbes [10]. Therefore, AMF can help plants cope with the adverse effects of warming through a variety of mechanisms. For example, AMF can increase the absorption capacity for water and nutrients as well as nutrient utilization efficiency [11], improve the photosynthetic rate [12], and improve the activity of antioxidant enzymes [13]. However, to date, it is still unclear how preceding crops inoculated with AMF under climate warming affect the growth and development of subsequent plants through soil legacy.
Rapeseed is one of the most important oil crops planted worldwide [14]. Soil warming promotes the growth of rapeseed at an early stage and during spring [15]. Although it is generally considered that Brassicaceae species are non-mycorrhizal plants, previous studies have shown that inoculation with AMF (mycorrhizal colonization rate: 33%-59%) significantly promotes the growth and yield of rapeseed [16]. Rape inoculated with the phosphorus-solubilizing bacterium as the preceding crop increased the shoot and root fresh weight of the succeeding plant, soybean [14]. However, it is unclear whether soil legacy affects the growth and reproduction of succeeding plants when rapeseed as a previous crop is inoculated with AMF under climate warming. Therefore, this study took oilseed rape as the previous crop, which was subjected to the treatment of warming and/or inoculation with AMF. Impatiens balsamina, as a subsequent plant, was grown in the post-harvest soil of rapeseed. The growth and reproductive characteristics of I. balsamina were measured to explore the soil legacy effects of inoculation with AMF under climate warming.
Materials and Methods
Study Site
This study was conducted in the experimental field of China West Normal University in Sichuan Province, China (106°03´16.33″E, 30°49´02.77″N, 307 m a.s.l.). This region has a humid subtropical monsoon climate, with an average annual temperature of 15.8ºC-17.8ºC, annual precipitation of 1020-1250 mm, average annual relative humidity of 78%-85%, and average annual sunshine duration of 1200-1500 h. The soil in this area is mainly calcareous, and the type is yellow soil [17].
Study Species
The previous crop was oilseed rape (Brassica napus L.), the variety of which was Jingjingyou 007, cultivated by Sichuan Xindi Seed Industry Co., Ltd., China. Garden balsam (Impatiens balsamina L.) was selected as the succeeding plant for several reasons. First, garden balsam is an important ornamental plant and is widely cultivated in gardens all over China [18]. Second, the species serves as a valuable candidate for soil restoration [19]. Third, garden balsam and oilseed rape have staggered growing periods, making them ideal for crop rotation. Garden balsam is an annual herb, 60-100 cm tall. Solitary or 2-3 fascicled flowers grow in the leaf axils, and flowers have no total pedicles with single or double lobes. Flowers have various colors, such as pink, red, purple, pink-purple, and so on [20]. In this study, a variety with red flowers was selected. This species blooms from July to October. The capsule is wide and spindle-shaped.
Experimental Design
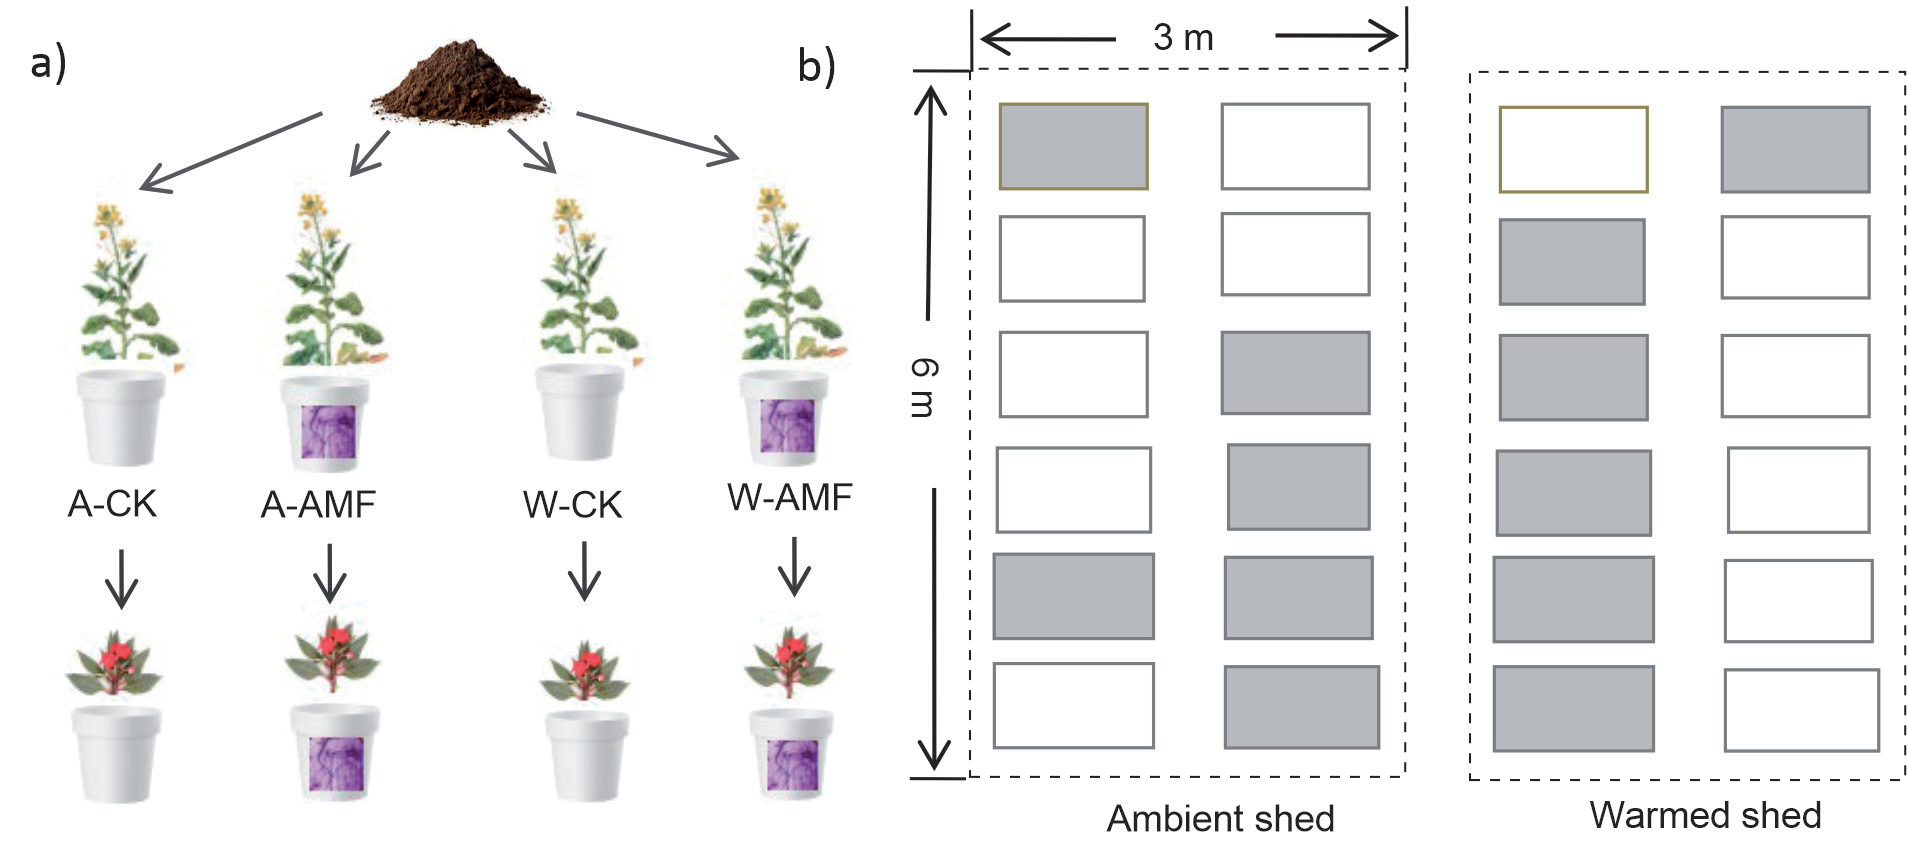
The entire experiment was designed with two factors (warming and inoculation with AMF). From November 2022 to May 2023, 144 seedlings of oilseed rape were randomly assigned to two temperature treatments (ambient vs. warmed). Two inoculation treatments were nested within warming treatments (inoculation with Funneliformis mosseae vs. inoculation with inactivated F. mosseae) (Fig. 1a)). Thirty-six rape seedlings were randomly assigned to six plots (6 pots per plot, 3 pots/row × 2 rows) for each experimental treatment (Fig. 1b)). A seedling was planted into a pot with a height of 30 cm and a diameter of 30 cm at the top of the pot. The warming treatment was achieved by a closed plastic greenhouse of 6 m × 3 m × 2.1 m, and the side film of another plastic greenhouse was rolled up, and the door of the greenhouse was opened to create the non-warming treatment. The temperature increase was 1.54ºC from March 8 to May 8, 2023. The distance between the two plastic greenhouses was 1.0 m. Each seedling of the inoculation treatment was inoculated with 10 g of the agent of F. mosseae. When inoculated with inactivated AMF, each seedling was inoculated with 10 g of agent after sterilization (121ºC sterilization for 30 min). The inoculant was purchased from the Root Biology Institute of Yangtze University, China. On April 22, 2023, full seeds of garden balsam with uniform size were selected, sterilized, and soaked, and then seeded in a seedling tray in a greenhouse. The culture medium of the seedling tray was nutrient soil. In May 2023, after all the rapes were harvested, garden balsam seedlings, which are 3 cm tall, robust, free of pests and diseases, and uniform in growth, were transplanted into pots, and the medium used in the pot was the rape soil left over from the previous crop. Finally, four to six plots for each treatment were selected as the experimental subjects in this study. These garden balsam seedlings were managed daily after transplanting. The side film of both plastic greenhouses was rolled up throughout the growth period, and they were covered with a black plastic sunshade with 80% light transmission from June 2023.
Fig. 1.
Schematic diagram of experimental design (a) and the layout of experimental plots (b). A, ambient temperature; W, warmed treatment; CK, without arbuscular mycorrhizal fungi inoculation; AMF, the inoculation with arbuscular mycorrhizal fungi. The whiteand gray-filled small rectangles represent the experimental plots without and with AMF inoculation, respectively.
Determination of Gas Exchange Characteristics
After the experimental plants of I. balsamina underwent over one month of acclimatization growth, on July 16, 2023, during the early blooming period of garden balsam, the gas exchange characteristics were measured from 8:00 to 10:30 a.m. on a sunny day using a portable photosynthesis measurement system (LI6400, Li-Cor Inc., Lincoln, NE, USA) with a standard LED leaf chamber (2 cm × 3 cm). The measurement was taken at the widest part of the third mature leaf from the top of the stem. The measurement conditions were as follows: flow rate of 500 μmol·s-1, leaf temperature of 25ºC, relative air humidity of 55%-60%, CO2 concentration of 350 ppm, and photosynthetic photon flux density (PPFD) of 1000 μmol·m-2·s-1. The gas exchange characteristics measured included net photosynthetic rate (Pn), stomatal conductance (Gs), intercellular CO2 concentration (Ci), and transpiration rate (Tr). Five plants were randomly selected for each treatment from at least three plots. One leaf of each plant was measured for five values, and the average of the last three values represented the gas exchange characteristics of the sample leaf to avoid disturbances caused by leaf chamber opening.
Determination of Chlorophyll Fluorescence Parameters
On July 21, 2023, chlorophyll fluorescence parameters of the third mature leaf from the top of the stem were measured using a chlorophyll fluorometer (Handy PEA, Hansatech Instruments Ltd., UK). Each selected leaf was dark-adapted for 25 min prior to measurement using a dedicated leaf clip. After adaptation, a saturating light pulse of 3,500 μmol (quanta)·m-2·s-1. was applied for 2 s, and the chlorophyll fluorescence parameters, such as initial fluorescence (Fo) and maximum fluorescence (Fm), were measured. Fluorescence rise kinetics O-J-I-P curves were drawn [21]. Five plants were randomly selected for each experimental treatment.
Measurement of Plant Height and Counting the Number of Flowers and Fruits
At the end of June 2023, the plant height of five randomly selected plants per experimental treatment was measured from the root neck to the top of the stem using a tape measure. In early September 2023, the number of flowers and fruits per plant was counted. From August to September 2023, ten nearly ripe fruits from each plant were randomly selected, and the number of seeds per fruit was counted. Five individual plants were randomly selected for each experimental treatment, and a total of 200 fruits were collected from 20 selected plants.
Determination of Soil Physical and Chemical Properties
Soil samples were collected in late October 2023 at the end of the growing season. After natural air-drying, the soil was preserved for subsequent analysis. In April 2024, the water content of air-dried soil was determined by the drying method; pH values of soil solutions were measured by the potentiometric method using a pH meter (PB-10, Sartorius, Germany). In May 2024, the soil organic matter content was determined by the hydrated thermal potassium dichromate oxidation-colorimetric method using a UV-visible spectrophotometer (752, Shanghai Jinghua Technology Instruments Co., Ltd., China) [22]. The soil carbon and nitrogen contents were measured using an element analyzer (Variotoc, Elementar, Germany), and the carbon-nitrogen ratio was calculated. Five soil samples were randomly measured for each experimental treatment.
Statistical Analysis
All statistical analyses were conducted using R4.3.2 [23]. The Shapiro-Wilk test (Stats package) and Levene’s test functions (Car package) were used to test the normality and homogeneity of residuals of the linear model, respectively. When the residuals of data met the normality and the variances were homogeneous, the data were fitted using linear models (LMs, no significant random effects) or linear mixed-effect models (LMMs, with stronger random effects). If not, the data were fitted using generalized linear models (GLMs, with weaker random effects) or generalized linear mixed-effect models (GLMMs, with stronger random effects). For Pn and Ci, linear mixed models (LMMs) were fitted using warming and inoculation with AMF as the predictors and plot identity (ID) as a random factor. Gs and Tr were analyzed using GLMMs with plotID or plantID nested within plot ID as a random factor. For Fo and Vi, we fitted Gamma GLMs. Fm and PI total were fitted using LMs. For Fv, Sm, PIinst., and PIabs., we fitted LMMs with plot ID or plant ID as a random effect. Fv/Fm, Fv/ Fo, and Vj were fitted with Gamma GLMMs with plot ID or plant ID nested within plot ID as a random factor. The number of seeds per fruit was analyzed using logit-link Poisson GLMM with plant ID as a random factor. The number of flowers per plant was analyzed using LMM, with plant ID nested within plot ID as a random factor. Plant height and number of fruits per plant satisfied normality and homogeneity of variances, so LMs were used for analysis. Soil carbon content was analyzed using Gamma GLMM with plant ID as a random factor. Soil pH values and soil C/N ratio were fitted using LM and Gamma GLM, respectively. Soil organic matter, soil water content, and soil nitrogen content were analyzed using LMMs with plant ID as a random factor. All these analyses were fitted in the lme4 package in R [24], and the significance of the experimental treatment effects was tested using the Anova function in the Car package. If the effect was significant, multiple comparisons were conducted using the emmeans package [25]. The box plots were drawn using the ggplot2 package, and the fluorescence kinetic curves were plotted in Excel.
Results and Discussion
Photosynthetic Physiological Characteristics
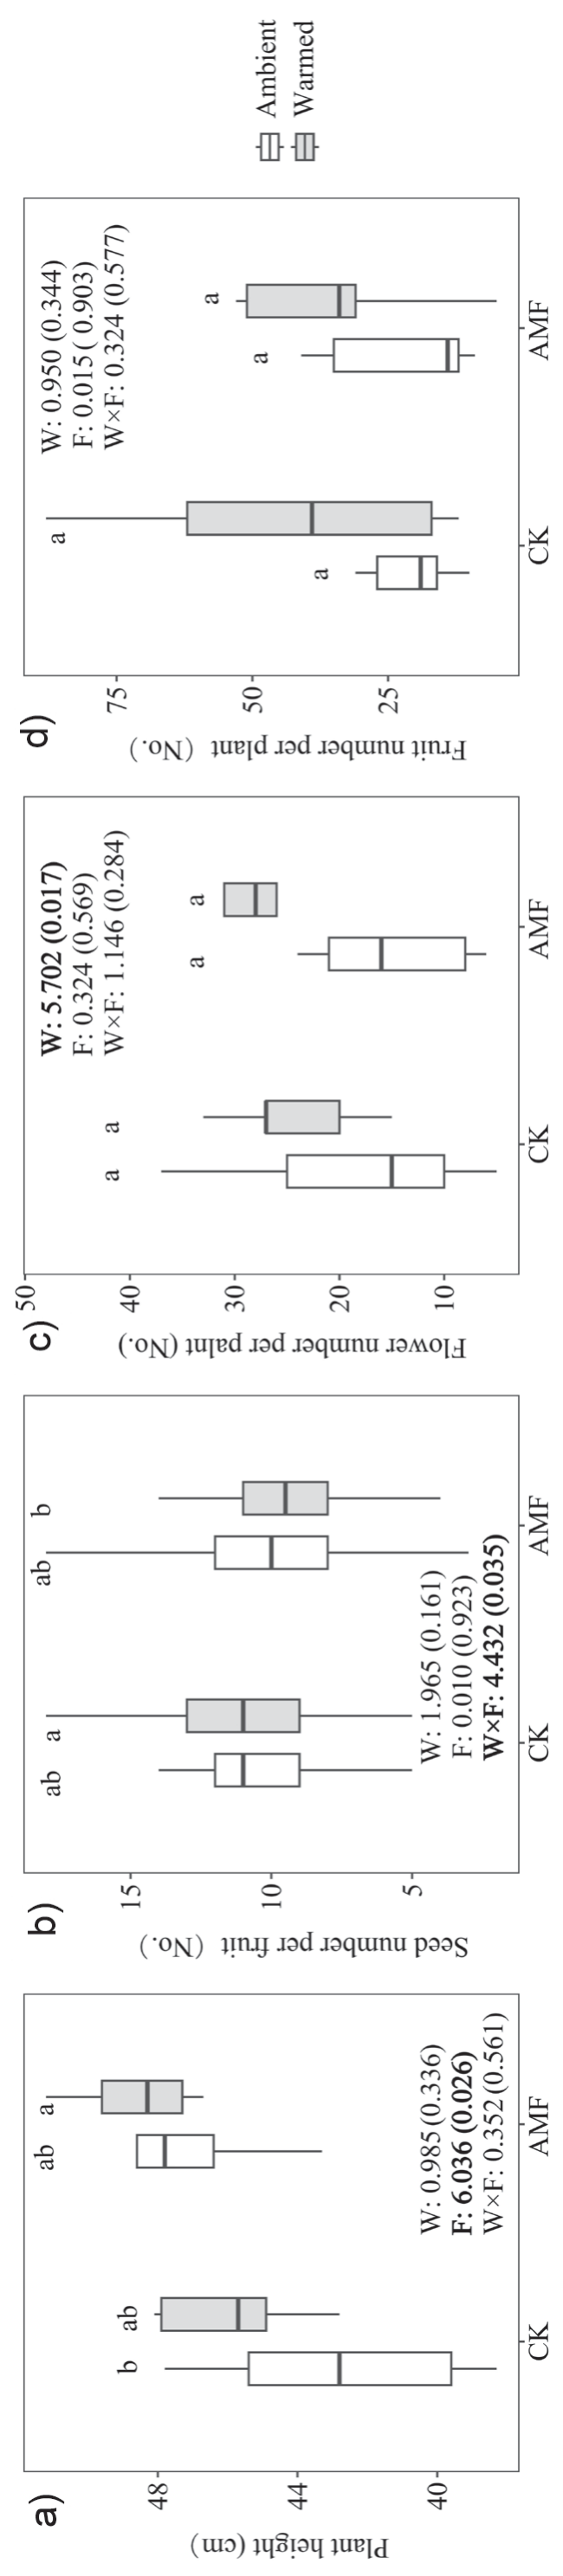
Soil legacy of rape driven by warming did not affect the net photosynthetic rate (Pn) and transpiration rate (Tr) of I. balsamina (Fig. 2a), d)), but significantly increased stomatal conductance (Gs) and intercellular CO2 concentration (Ci) by 54.5% and 1.7%, respectively (Fig. 2b), c)). Soil legacy of rape inoculated with AMF significantly decreased stomatal conductance (Gs), intercellular CO2 concentration (Ci), and transpiration rate (Tr) of I. balsamina by 53.4%, 4.47%, and 46.5%, respectively (Fig. 2b), c), d)). The interaction effects driven by warming and inoculation with AMF of the previous crop of rape did not affect the four gas exchange characteristics of I. balsamina. In addition, the two factors did not significantly affect some chlorophyll fluorescence parameters of I. balsamina, such as Fo, Fm, Fv, Fv/Fm, Fv/Fo, and PItotal (Table 1). When the previous crop rapes were not inoculated with AMF, there was no significant difference in Vj, Sm, PIinst., and PIabs of I. balsamina grown in the soil between ambient and warmed treatments. In contrast, Sm, PIinst., and PIabs of I. balsamina from the soil legacy of rape under ambient environment were significantly higher than those under warmed treatment when the previous rapes were inoculated with AMF (Table 1). Sm, PIinst., and PIabs of I. balsamina grown in the soil from ambient environment and AMF inoculation were significantly higher than those from warming and AMF inoculation as well as from ambient environment and non-AMF inoculation, because more light energy was being dissipated as fluorescence rather than driving photochemistry (Table 1, Fig. 3a), b)). The soil legacy from the warming treatment significantly enhanced Gs and Ci of I. balsamina, but increased Vj and decreased Sm. These results indicated that electron transfer in the photosynthetic chain was impaired, thus resulting in similar net photosynthetic rate and PI total. Moreover, due to the relatively weak dependence of Impatiens species on AMF [26], garden balsam grown in soil inoculated with AMF did not improve its photosynthesis. In addition, previous crops can lead to the occurrence of soil-borne diseases and toxicity under higher temperatures, thus reducing the net photosynthetic rate and dry matter accumulation of succeeding plants [27].
Plant Height, Flowering, and Fruiting
Garden balsam grown in legacy soil of rape inoculated with AMF had a significant 7.8% increase in plant height (Fig. 4a)), but had no significant change in flower number and fruit number (Fig. 4c), d)). At the end of flowering, the number of flowers per plant in the warmed conditions was 61.1% higher than that in the ambient conditions (Fig. 4c)). In addition, only under the warmed conditions was the number of seeds per fruit in legacy soil of rape inoculated with AMF 17.5% lower than that without inoculation with AMF (Fig. 4b)). Soil legacy of rape inoculated with AMF promoted the height growth of garden balsam for five main reasons. First, it is possible that the microbial soil legacy, including AMF, can increase the total chlorophyll content of plants by increasing the uptake of Mg to enhance the photosynthetic capacity [28]. Second, AMF significantly promote the degradation of rape straw and the release of mineral nutrients, increasing the content of available nutrients in soil [29]. Third, AMF in soil legacies can increase soil aggregation [30]. Fourth, AMF can induce tolerance in I. balsamina against root diseases caused by pathogens [31]. Finally, AMF in soil legacies can colonize the roots of I. balsamina, facilitating nutrient (e.g., P) and water acquisition of plants [32]. Life history strategy theory holds that there is a trade-off between vegetative growth and sexual reproduction [33]. Therefore, an increase in plant height resulted in a reduction in the allocation to sexual reproduction (fewer seeds per fruit) under inoculation with AMF. In our study, garden balsam grown in post-rapeseed cultivation soil exposed to warming significantly increased flower number at the end of flowering, possibly because warming promoted the release of root exudates and soil carbon input [34] or the decomposition of organic matter [35], thus improving soil nutrient availability. Elevated temperatures can restrict plant growth, decrease plant dependence on AMF, reduce the nutrient supply to AMF, and thus change the life history strategy of AMF [36]. On the other hand, warming promotes the decomposition of soil nutrients, leading to an increase in soil effective nutrient content, which is conducive to the stability of soil AMF community diversity [37]. These results show that plant-soil-AMF interactions are very complex in the context of global warming.
Fig. 2.
Soil legacy effects of rape grown in warming and/or AMF inoculation on the gas exchange characteristics of I. balsamina. W, effect of warming; F, effect of inoculation with AMF; W×F, the interaction of the two factors. The bold font indicates a significant effect at the P<0.05 level. The values in parentheses indicate the significance probability (P-value).
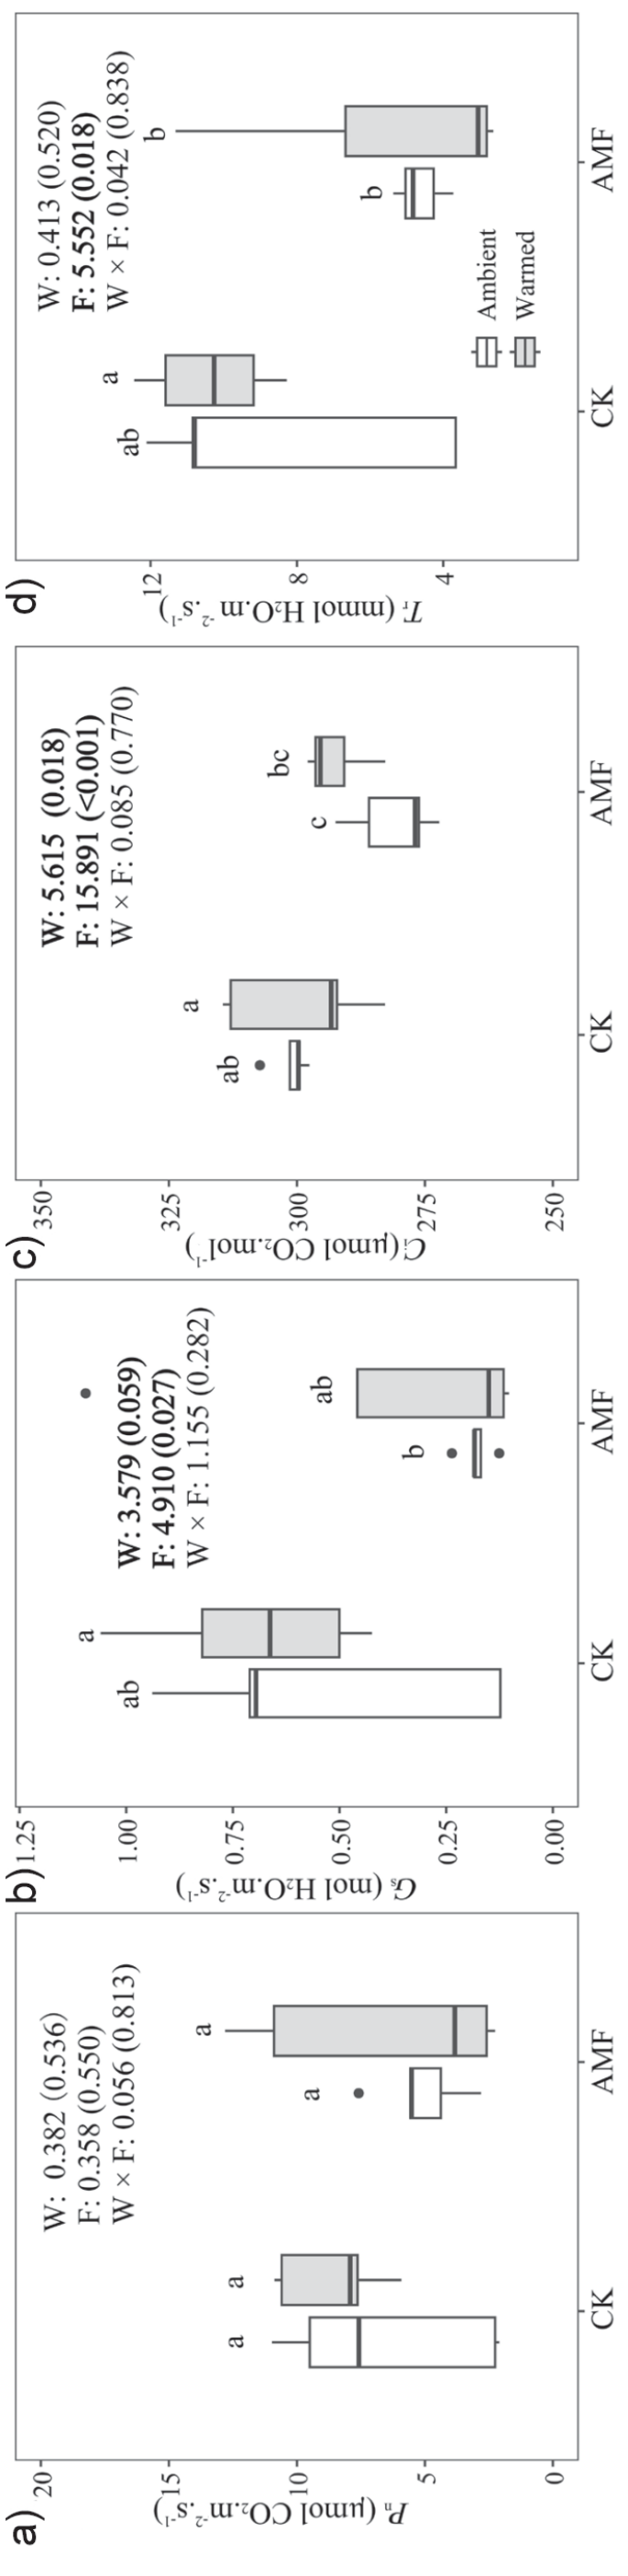
Fig. 3.
Chlorophyll fluorescence kinetic curves of I. balsamina under different soil legacy driven by warming and inoculation with AMF. ΔVt, differences in relative variable fluorescence, ΔVt = Vt (treatment) – Vt (control). Control, soil legacy driven by ambient environment, and no AMF inoculation.
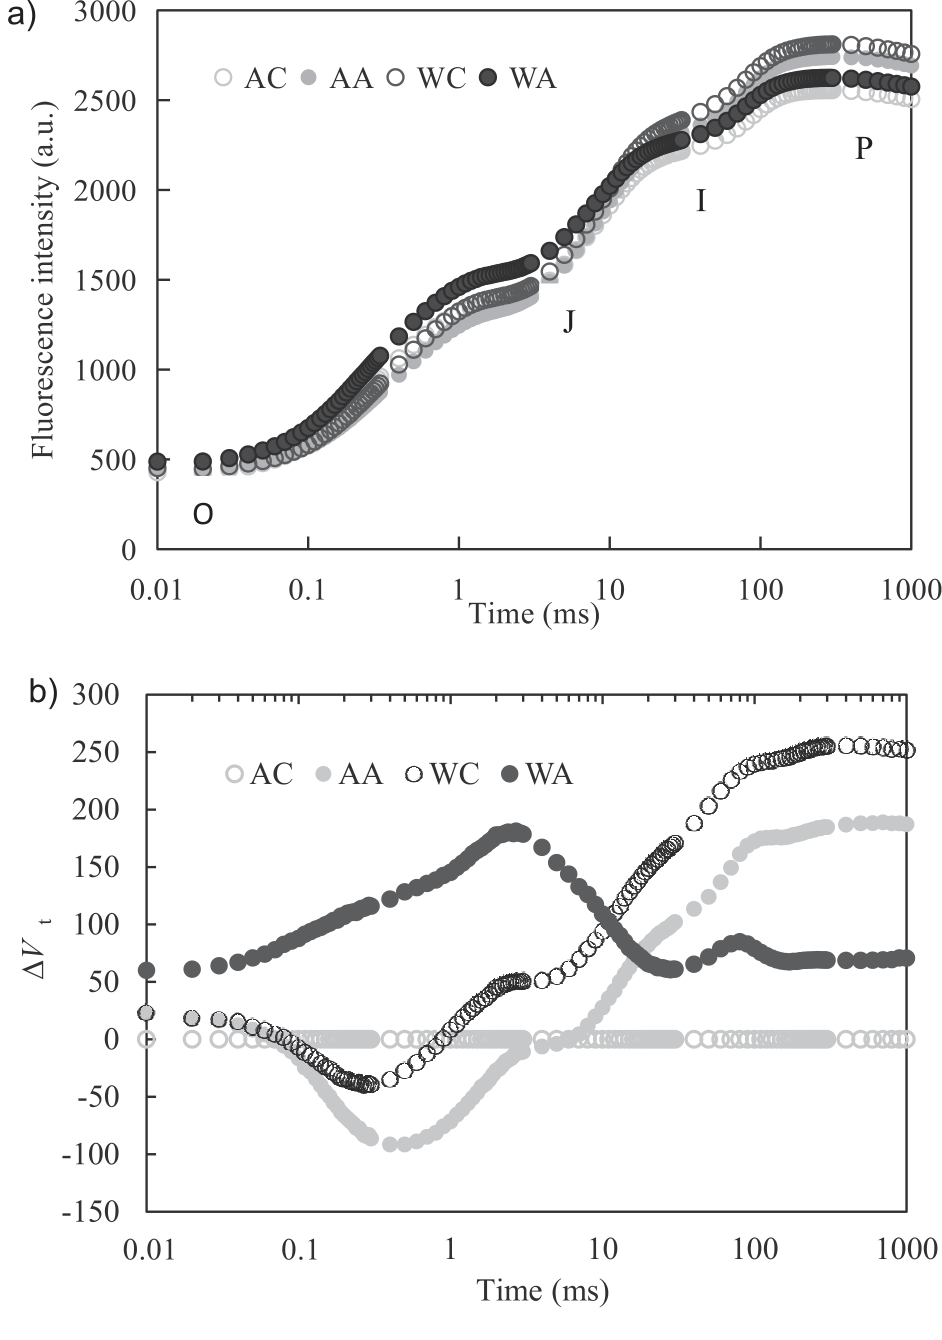
Table 1.
Soil legacy effects of rape grown under warming and/or AMF inoculation on chlorophyll fluorescence parameters of I. balsamina. The same lowercase letters in the same line represent no significant difference in mean among the four treatments, the last three columns are chi-square or F values, and the values in parentheses indicate the probability of significance.
[i] Fo, minimal fluorescence; Fm, maximal fluorescence; Fv, maximal variable fluorescence; Fv/Fm, maximum photochemical efficiency of PSII; Fv/Fo, potential activity of PSII; Vj, relative variable fluorescence at the J-step; Vi, relative variable fluorescence at the I-step; Sm, normalized total complementary area above the O-J-I-P transient (reflecting multiple-turnover QA reduction events); PIinst., instantaneous performance index; PIabs, performance index on absorption basis; PItotal, performance index on a total chlorophyll basis.
Table 2.
Soil legacy effects of rape grown under warming and/or AMF inoculation on the soil physicochemical properties of I. balsamina. The same lowercase letters in the same line represent no significant difference in mean among the four treatments, the last three columns are chi-square or F values, and the values in parentheses indicate the probability of significance.
Physical and Chemical Properties of Soil
The soil legacy of previous crops of rapeseed grown in warming and/or inoculation with AMF conditions had no significant effects on soil organic matter content, pH value, water content of air-dried soil, and soil nitrogen content (Table 2). However, the soil legacy of the previous crop, rapeseed inoculated with AMF, significantly increased the soil carbon content by 16.2% compared to that of the uninoculated AMF under warming (Table 2). This is because AMF promoted the growth of I. balsamina at the early stages, which in turn enhanced the production of root exudates. Overall, the C/N ratio of the soil from the warming treatment increased significantly by 7.8% compared to that of the soil from ambient conditions (Table 2). Plants exposed to warming can increase their root exudation rates [38] or promote the decomposition of organic matter [37], similar to the effects of warming on the flower number of I. balsamina.
In our study, the previous crop, rapeseed, and subsequent plant garden balsam were cultivated for only one season, and the effects of climate warming are long-term and slow; follow-up studies should be conducted in the future. Under warming and AMF treatment, the soil legacy effects of rapeseed on the reproduction of I. balsamina may be achieved through affecting pollination; thus, soil legacy effects on plant-pollinator interactions should be further studied. The photosynthetic physiological characteristics of garden balsam were only determined in the early stage of flowering. Other developmental stages should be determined to reveal the mechanism of soil legacy effects more fully.
Conclusions
Soil legacy of rape inoculated with AMF promoted the plant height of I. balsamina because the improved PSII functionality offset the decline in Ci due to the lower stomatal conductance. The increase in vegetative growth also led to a reduction in the number of seeds per fruit. Warming-driven soil legacy significantly increased Ci and decreased PSII electron transfer efficiency but did not significantly affect Pn and plant height of I. balsamina. Flower number per plant and soil C/N ratio were enhanced by warming-driven soil legacy. Collectively, the soil legacy of rape inoculated with AMF had positive effects on the vegetative growth in early stages but had negative effects on the seed production of I. balsamina, particularly in warming-driven legacy soils.

