

Introduction
Severe rocky desertification and soil erosion, frequent occurrences of droughts and floods, recurrent karst collapses, and the degradation of groundwater quality constitute the most urgent ecological challenges currently facing karst regions [1]. Since the early 21st century, these challenges have been central to the focus of karst researchers. Considering the inherent features of rocky desertification regions – characterized by high rock exposure, limited and shallow soil presence, soil aridity, and increased calcium levels [1, 2] – plants selected for mitigating karst desertification must possess drought tolerance, lithophilous properties, a preference for calcium, and strong, well-developed root systems. Multiple studies have evidenced that climbing plants exhibit significant adaptability, rapid growth, and extensive root systems due to their capability to grow by adhering to supports such as rocks, other vegetation, and cliffs. These plants are distinguished by their substantial biomass, minimal ground space requirements, extensive coverage, and inherent mobility and resilience to degradation [3, 4]. These traits allow them to rapidly establish vegetation cover in rocky desertification regions. Additionally, some climbing plants possess specialized structures like aerial roots and adhesive discs [3], which effectively mitigate soil erosion and enhance soil stabilization and water retention, thereby attracting considerable interest in managing rocky desertification. Consequently, investigating the precise mechanisms through which climbing plants mitigate rocky desertification in karst regions is of notable importance. Future studies should concentrate on these plants’ ecological adaptability, their interactions with soil microorganisms, and their capacity to improve soil structure and moisture retention. Such research will offer a more robust scientific foundation and efficacious practical strategies for ecological restoration in karst areas. Investigating the lianas’ community structure and functional diversity will elucidate their adaptive strategies across diverse ecological niches. What’s more, exploring their symbiotic interactions with other plant species may yield new insights into improving the efficiency of vegetation restoration. The systematic application of advanced biotechnology to refine lianas’ cultivation and transplantation methods will further enhance ecological restoration efforts in karst regions. In China, climbing plants are represented by 85 families, 409 genera, and 3,037 species, with over 50% occurring in rocky desertification zones [5]. Among these, species such as honeysuckle, trumpet vine, ivy, common milletia, Virginia creeper, Xueli, cliff bean vine, thunderbolt vine, passionflower, kudzu, and solanum are considered pioneer species for ecological restoration efforts in these regions [6, 7]. Nevertheless, due to insufficient attention, suboptimal management, and a lack of comprehensive research, developing a highly effective model or methodology for utilizing lianas in rocky desertification control remains unachieved. Consequently, identifying lianas with robust adaptability, rapid growth, resilient vitality, substantial medicinal value, and considerable economic benefits is of both theoretical and practical significance for vegetation restoration and reconstruction in karst areas.
The non-karst-adapted plant, N. grossedentata, a perennial woody vine belonging to the Vitaceae family, prospers in valley regions or shrublands situated on mountain slopes, utilizing tendrils to climb and secure itself to other trees [8, 9]. It is ideally suited for intercropping within shrublands or forested areas. Various studies have demonstrated that the optimal planting density for N. grossedentata is 1,500 plants per mu, yielding tender leaves at 760.5 kg/hm2 and common leaves at 6,159.0 kg/hm2 [10]. Moreover, N. grossedentata is rich in flavonoid compounds such as dihydromyricetin, myricitrin, and myricetin [11, 12]. The dried leaves possess a total flavonoid content reaching up to 45.52%, with dihydromyricetin comprising 39.50%, thus garnering the designation “King of Plant Flavonoids” [13]. Contemporary pharmacological investigations have demonstrated that N. grossedentata exhibits a range of pharmacological activities, including antibacterial, anti-inflammatory, blood-sugar-lowering, lipid-lowering, blood pressure-reducing, antioxidant, anti-atherosclerotic, liver-protective, and anti-tumor effects [13, 14]. In summary, N. grossedentata possesses the following advantages: strong environmental adaptability, a well-developed root system, and vigorous growth; rapid growth with high leaf yield; significant medicinal value, promising market potential, and substantial development prospects. To date, research on its cultivation has primarily focused on its growth and development, morphological characteristics, and physiological and biochemical properties. However, the optimal growth conditions for N. grossedentata in karst soils and its adaptation mechanisms to such environments remain unclear. Furthermore, there is a lack of literature on its response mechanisms and the dynamics of secondary metabolite content under karst conditions. This study employs high-performance liquid chromatography to analyze the leaves of N. grossedentata growing in native soil, dolomite, and limestone-attached soils, tracking the dynamic changes of key functional components such as dihydromyricetin, myricitrin, and myricetin within the leaves. Simultaneously, ultraviolet spectrophotometry was utilized to study the physiological and biochemical changes in chlorophyll and soluble sugars, while atomic absorption spectrophotometry was employed to analyze variations in calcium content within the plant leaves. These findings contribute to a systematic elucidation of N. grossedentata’s adaptive mechanisms in karst soils, its response mechanisms in karst environments, and the changes in secondary metabolite content. This research offers new insights into species selection in karst stony desertification control. It lays the theoretical foundation and technical support for using non-karst-adapted N. grossedentata in stony desertification restoration.
Materials and Methods
Test Materials
The experiment was conducted in the experimental greenhouse at Guizhou Normal University. N. grossedentata from Guangnan, Yunnan (YNGN); Jinxiu, Guangxi (GXJX); and Honghe, Yunnan (YNHH) were selected. The experimental soils included native soil, dolomite-attached soil, and limestone-attached soil.
The dolomite-attached soil, limestone-attached soil, and native soil of N. grossedentata were all excavated from Huaxi District, Guiyang City, Guizhou Province. Soil samples tested by Chun Feng [15] revealed that the native soil is slightly acidic, with total calcium and soluble calcium measuring 0.37 g/kg and 72.80 mg/kg, respectively. The karst-attached soil was characterized as slightly alkaline, with dolomite-attached soil exhibiting total calcium and soluble calcium concentrations of 34.94 g/kg and 113.77 mg/kg, respectively, while limestone-attached soil demonstrated total calcium and soluble calcium levels of 75.60 g/kg and 166.51 mg/kg, respectively (Table 1).
Table 1.
Longitude, latitude, elevation, pH, total calcium, and soluble calcium content in different soils.
Test Design
N. grossedentata specimens were selected from three distinct genetic backgrounds: Guangnan, Yunnan (YNGN); Jinxiu, Guangxi (GXJX); and Honghe, Yunnan (YNHH). Prof. Chºººong Luo of the School of Life Sciences at Guizhou Normal University identified the plant. From each genetic background, three mother plants were selected, and each was subsequently divided into three parts, yielding independent plants approximately 15 cm in height with consistent growth vigor. In total, 27 plants were utilized. Each pot, measuring 30 cm in upper diameter, 20 cm in height, and 20 cm in lower diameter, was filled with 10 kg of soil, and transplantation took place before the Qingming Festival in 2019. Transplantation was conducted on a cloudy day, with all leaves pruned from the plants to reduce transpiration. In addition to preserving differences in soil conditions, consistency in natural conditions such as climate, temperature, and light must be ensured.
Determination of Physiological and Biochemical Indexes
Sampling was conducted before 9:00 on June 17, 2023. All mature leaves were pruned two weeks prior to sampling, and samples were evenly taken from the upper, middle, and lower sections. After removing the main veins, the leaves were placed in an oven and dried to a constant weight at 60ºC, then ground to a fine powder and passed through an 80-mesh sieve for future use.
The functional components (dihydromyricetin, myricetin, and myricitrin) were determined using high-performance liquid chromatography, with modifications based on the method [16]. An ultrasonic method to extract total compounds from leaves was used. Approximately 10.00 mg of oven-dried leaf tissue was weighed per sample and placed into a centrifuge tube, to which 5.00 mL of methanol extract was added. After shaking evenly, filter to obtain the test solution. The compound concentrations were determined using high-performance liquid chromatography (HPLC), employing methanol as solvent A and 0.1% phosphoric acid as solvent B, with the following gradient: 0 min at 26:74, 10 min at 50:50, 15 min at 55:45, and 25-30 min at 26:74. The column was maintained at 40ºC, with a sample injection volume of 5.0 µL and a flow rate of 1 mL/min. Detection wavelengths were set at 292, 254, and 375 nm.
Chlorophyll was measured using the 80% acetone ultrasonic method [17]. Sample and weigh the N. grossedentata (dry sample, 6.00 mg), then place it in labeled test tubes. Using a pipette, add 2.00 ml of 80% acetone solution to each tube and perform ultrasonic extraction for 30 min. After 30 min, measure the absorbance at 663 nm and 646 nm using 80% acetone as the blank and record the data. After the determination, the chlorophyll content was calculated according to the following formula:
Ca+b = 20.29A645 + 8.05A663
Chlorophyll content (mg/g) = Ca+b*V/W
Meanwhile, soluble sugars were assessed using the “phenol-sulfuric acid” colorimetric method [18]. The calcium content in plant leaves was analyzed using atomic absorption spectrometry, entrusted to Guizhou Bailoni Testing Technology Co., Ltd [19].
Data Analysis
All data were processed with GraphPad Prism 10 to make a histogram. Data analysis was conducted using SPSS 20.0 and Origin 2024 software, employing one-way ANOVA to compare the significant differences in physiological and biochemical changes of N. grossedentata across different soils (P<0.05). The Pearson correlation coefficient denotes the degree of correlation, with * indicating significance at the 0.05 level and ** indicating high significance at the 0.01 level.
Results and Discussion
The Primary Active Components of N. grossedentata under Three Distinct Soil Conditions
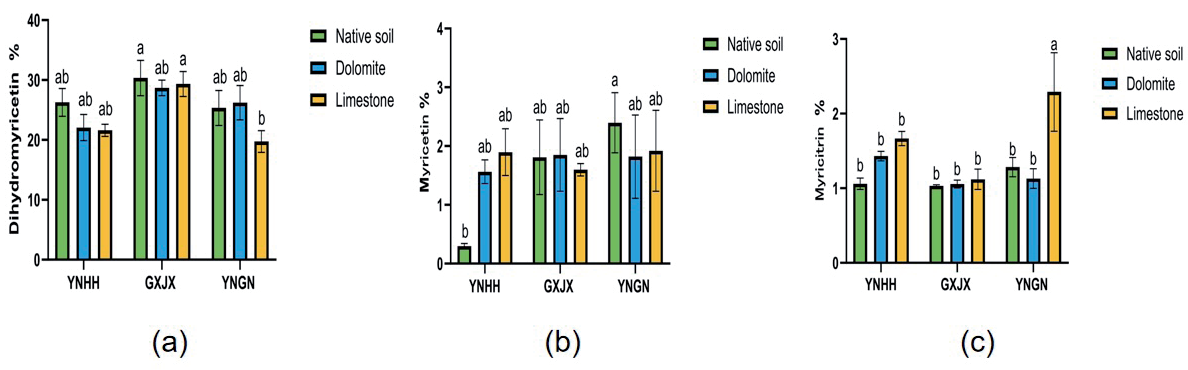
As depicted in Fig. 1a), the concentration of dihydromyricetin in GXJX remains nearly equivalent to that in native soil, while in YNGN, the content in dolomite slightly surpasses that of native soil, with limestone showing the lowest levels. In YNHH, the dihydromyricetin content declined with increasing calcium levels in the soil, yet no significant differences were observed (P>0.05). Overall, the variation of dihydromyricetin in N. grossedentata across the three soil types was minimal. In YNHH, dihydromyricetin peaks at 27.79±3.67% and falls to a low of 21.60±1.03%, marking a decrease of 6.19%. In GXJX, the native soil group (30.33±2.95%) surpasses the limestone group (29.34±2.08%), which in turn exceeds the dolomite group (28.68±1.30%). In YNGN, the dolomite group registered the highest content (26.22±2.87%), followed by the native soil group (25.34±2.92%), with the limestone group trailing at 19.73±1.82%. In YNHH, as the calcium content in the soil increases, the myricetin concentration shows a gradual upward trend, with the limestone group (1.90±0.40%) surpassing the dolomite group (1.57±0.20%), which in turn exceeds the native soil group (0.30±0.04%); the dolomite and limestone groups exhibit increases of 5.25 and 6.37 times over the native soil group, respectively (Fig. 1b)). Conversely, in GXJX, the myricetin content across the three types of soil cultivation remained nearly uniform, with a slight elevation in the dolomite group, displaying no significant differences (P>0.05). In YNGN, the native soil exhibited the highest myricetin content (2.39±0.51%), followed by limestone (1.92±0.69%), with dolomite registering the lowest (1.82±0.71%), yet no significant differences were observed. In the genetic backgrounds of YNHH and GXJX, as the calcium content in the soil increases, the myricitrin content exhibits a gradual upward trend. In YNHH, the sequence is limestone group (1.67±0.09%) > dolomite group (1.35±0.03%) > native soil group (1.24±0.16%). In GXJX, it follows the limestone group (1.12±0.14%) > dolomite group (1.05±0.05%) > native soil group (1.03±0.02%) (Fig. 1c)). However, in YNGN, except for a slightly lower myricitrin content in the dolomite group compared to the native soil, the myricitrin content in the limestone group is 1.78 times that of the native soil group. This indicates that the calcium stress environment has a certain promoting effect on the accumulation of flavonoids, especially myricetin, in N. grossedentata, which may provide a new regulatory direction for accumulating functional components in N. grossedentata in specific environments. In conclusion, in N. grossedentata across three genetic backgrounds, the myricitrin content generally increases with higher soil calcium content, except in YNGN, where the dolomite content is slightly lower than in native soil.
In summary, under controlled experimental conditions, the accumulation of the primary functional component, dihydromyricetin, in N. grossedentata is influenced by its genetic background. However, in plants with inherently high dihydromyricetin content, the impact of soil calcium ions is minimal. The myricetin content does not exhibit a clear pattern. N. grossedentata growing in karst soils generally exhibits higher myricitrin content than in native soils. Flavonoids can be increased under environmental stress [20, 21]. Flavonoids are important for plant resistance to stress conditions [22]. A notable finding is the increase in myricitrin levels with higher soil calcium content. Secondary metabolites like flavonoids (e.g., dihydromyricetin, myricetin, and myricitrin) are known to play a crucial role in stress responses by acting as antioxidants, protecting plant cells from oxidative damage induced by calcium stress. This suggests that N. grossedentata leverages its secondary metabolism to counteract the potential oxidative and physiological disruptions caused by excessive calcium. GXJX inherently possesses a higher dihydromyricetin content than YNHH and YNGN. Under the three different soil conditions, the dihydromyricetin content in GXJX remains nearly equivalent to that in native soil, indicating that the accumulation of dihydromyricetin in N. grossedentata is tied to its genetic background, yet it is not significantly affected by soil calcium ion content in those with naturally higher dihydromyricetin levels. Myricetin content does not follow a discernible pattern. Throughout the growth and development process, plants cultivated in karst soils generally exhibit higher levels of the primary active component, myricitrin, than those grown in native soils. The variation in the content of active components corresponds to different genetic backgrounds, yet most plants experience a significant increase in myricitrin content when soil calcium content is moderately elevated. This indicates that when an increase in the beneficial compound myricitrin is desired, we can moderately enhance the content of exogenous calcium ions to promote plant absorption, thereby boosting myricitrin levels. The functional components (dihydromyricetin, myricetin, and myricitrin) are key indicators for assessing whether N. grossedentata is under stress conditions. Nonetheless, factors such as sample origin, soil properties, developmental stage, and individual variability persist, and their relationship with the content of active components in N. grossedentata leaves necessitates further investigation.
Variations in Chlorophyll Content and Soluble Sugars of N. grossedentata across the Three Soil Types
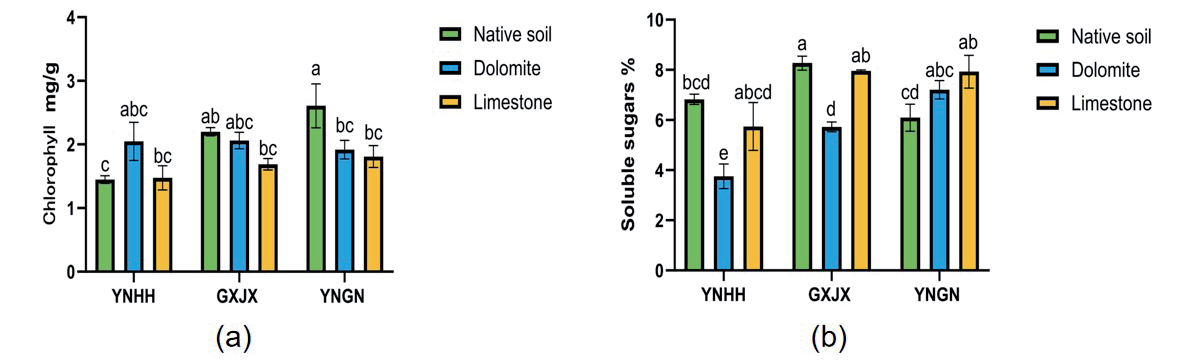
According to the data presented in Fig. 2a), with the exception of YNHH, chlorophyll content in samples from the other two genetic backgrounds decreases as soil calcium content increases. In GXJX, the native soil group (2.20±0.07 mg/g) surpasses the dolomite group (2.06±0.13 mg/g) and the limestone group (1.69±0.09 mg/g), with reductions of 0.14 mg/g and 0.51 mg/g, respectively, for dolomite and limestone compared to native soil (P>0.05). In plants with the YNGN genetic background, the native soil group (2.61±0.35 mg/g) exceeds the dolomite group (1.92±0.15 mg/g) and the limestone group (1.81±0.17 mg/g), showing significant differences with reductions of 0.69 mg/g and 0.80 mg/g for dolomite and limestone, respectively (P<0.05). In YNHH, the dolomite group registered a chlorophyll content of 2.05±0.30 mg/g, marking the highest among the three soil types within this genetic background. Considering the stable cultivation environment and experimental conditions, it can be inferred that the unique situation observed in YNHH is attributable to its genetic characteristics. When N. grossedentata effectively adapts to calcium ions, it can utilize exogenous calcium to maintain its osmotic pressure, leading to a reduction in chlorophyll content.
Soluble sugars are one of the critical factors for plants in maintaining osmotic pressure balance within their tissues [23, 24]. As illustrated in Fig. 2b), in plants with the genetic backgrounds of YNHH and GXJX, the content of soluble sugars is significantly reduced in dolomite compared to native soil and limestone, with significant differences (P<0.05). In YNHH, dolomite decreased soluble sugars by 3.07% compared to native soil and 1.08% compared to limestone. Similarly, in GXJX, the soluble sugar content in dolomite is 2.55% and 2.23% lower than in the native soil and limestone, respectively. In contrast, YNGN displays a gradual upward trend, differing from the other two genetic backgrounds. Besides genetic differences, this observation suggests that in response to environmental stress, plants may need to increase soluble sugar content to maintain cellular osmotic balance. However, stress conditions might lead to damage in plant leaf organs, which could restrict small molecule synthesis pathways, resulting in a decrease in soluble sugar content.
Chlorophyll and soluble sugars serve as indicators that are susceptible to change when plants respond to external environmental stresses [25, 26]. They play an important role in the resistance to environmental stress [27]. Environmental stress can disrupt chlorophyll synthase activity, inhibit chlorophyll synthesis, and enhance the activity of chlorophyll-degrading enzymes, leading to increased chlorophyll decomposition and, consequently, lower chlorophyll content [28]. Chlorophyll is a critical material basis for influencing plant photosynthesis. Under adverse conditions like high temperature, drought, and intense light, plants may experience membrane lipid peroxidation. In addition, plants can resist environmental stress by greatly increasing the content of soluble sugars and maintaining the balance of intracellular osmotic pressure [29]. In varying calcium ion environments, N. grossedentata exhibits significant differences in the stress resistance indicators of chlorophyll and soluble sugars (P<0.05), indicating that the plant indeed experiences stress upon increased calcium ion levels. However, these variations did not lead to plant mortality; instead, the plants adapted and flourished, leading to an increase in their functional substances. This illustrates the plants’ adaptability and tolerance to environments with elevated calcium ion concentrations compared to their native soil.
Variation in Total Leaf Calcium Content of N. grossedentata under Three Different Soil Conditions
According to the data in Fig. 3, with the exception of GXJX, the leaves of N. grossedentata with YNHH and YNGN genetic backgrounds showed an upward trend in total calcium content as soil calcium increases (P>0.05). In YNHH, the limestone group (2.64±0.09%) surpasses the dolomite group (2.14±0.23%) and the native soil group (1.74±0.30%), with increases of 0.40% and 0.90% for dolomite and limestone, respectively, compared to native soil. In YNGN, the limestone group (2.18±0.14%) exceeds the dolomite group (1.75±0.23%) and the native soil group (1.51±0.26%), with increases of 0.24% and 0.66% for dolomite and limestone, respectively. When plants find themselves in calcium-rich soil environments, calcium ions continually infiltrate the plant due to transpiration [30, 31]. The elevation of calcium content in both the soil and within the plant does not lead to plant mortality, highlighting N. grossedentata’s resilience and adaptability to environments rich in calcium ions.
Apart from plants with the GXJX genetic background, other groups show an increase in leaf calcium content with rising external calcium levels. This result suggests that N. grossedentata possesses a certain ability to absorb external calcium. In calcium-rich soil environments, calcium ions continuously enter the plant due to transpiration. However, the increase in calcium content in both soil and plants does not lead to plant mortality, demonstrating N. grossedentata’s tolerance and adaptability to calcium ion environments. High calcium content is a typical characteristic of karst soil environments [32]. Although calcium is crucial for plant growth and development, excessive calcium can be highly toxic, affecting plants’ absorption of other elements and reducing the soil’s nutritional value [33]. Therefore, N. grossedentata holds promise for mitigating high calcium stress on other plants in the soil, offering insights and practical applications for restoring karst environments. Additionally, as an important plant source for vine tea, it has the potential to develop high-calcium, high-flavonoid functional health products. N. grossedentata can be integrated into agroforestry systems, where it can stabilize soils while providing economic benefits by harvesting its leaves for medicinal and health products.
Correlation Analysis between Physiological and Biochemical Indicators of N. grossedentata and Soil Factors
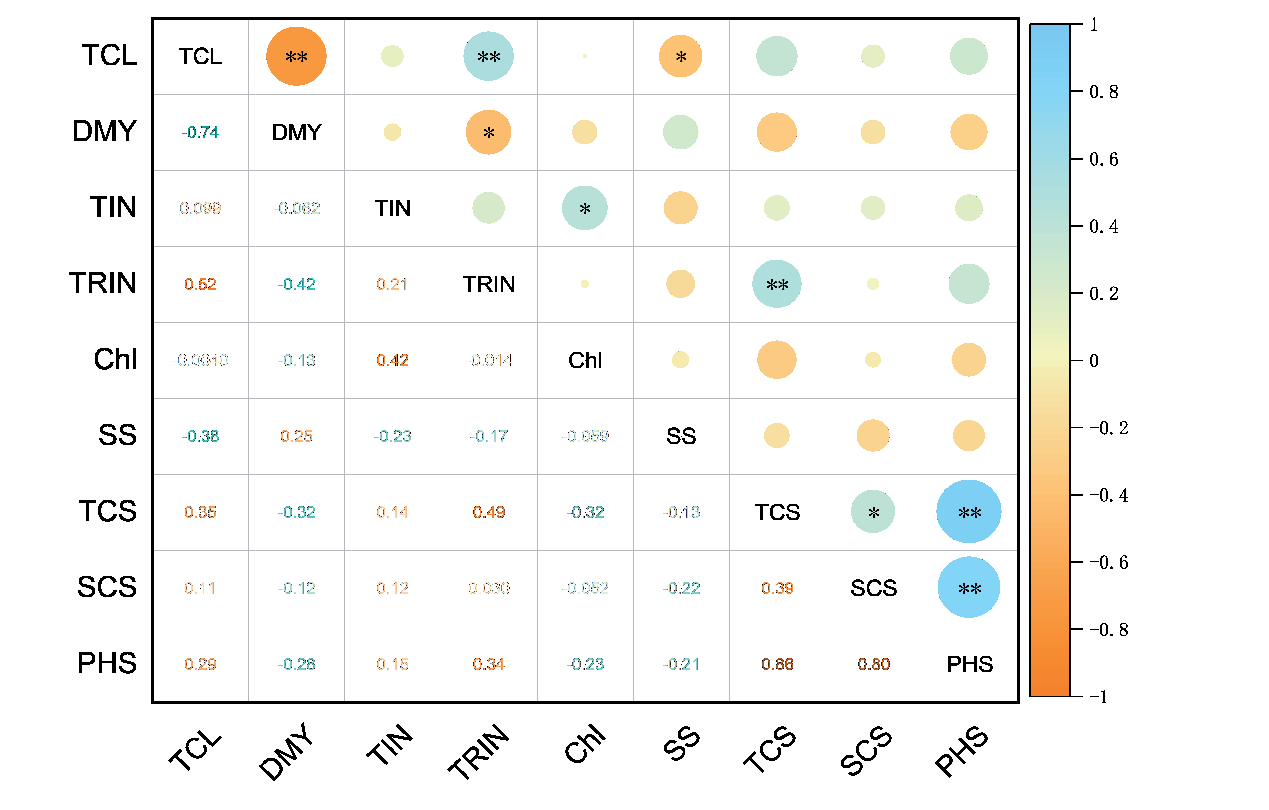
The analysis results of the Pearson correlation coefficient (Fig. 4.) reveal that total soil calcium exhibits a positive correlation with total leaf calcium, myricetin, and myricitrin while showing a negative correlation with dihydromyricetin, chlorophyll, and soluble sugar. Notably, myricitrin displayed a highly significant positive correlation with total soil calcium at the 0.01 level. Soluble soil calcium was positively correlated with total leaf calcium, myricetin, and myricitrin, and negatively correlated with dihydromyricetin, chlorophyll, and soluble sugar. Soil pH shows a positive correlation with total leaf calcium, myricetin, and myricitrin and a negative correlation with dihydromyricetin, chlorophyll, and soluble sugar.
This experiment aims to investigate the impact of high-calcium karst soil on the physiological and biochemical responses of N. grossedentata. Due to the genetic differences in N. grossedentata, varying calcium content in the soil may elicit diverse physiological and biochemical responses. The Pearson linear correlation coefficient analysis revealed a highly significant positive correlation between total soil calcium and myricitrin levels in the leaves of N. grossedentata at the 0.01 significance level. This suggests that to enhance the production of the functional compound myricitrin in N. grossedentata, we can moderately increase the concentration of external calcium ions for the plant to absorb. The correlation between various physiological indices of N. grossedentata under different soil calcium conditions is related to its resistance mechanisms under calcium stress. Furthermore, in karst regions, in addition to the critical issue of rocky desertification, associated challenges such as drought, severe soil water loss, and impoverished biological communities present significant threats to plant growth [34]. Therefore, future research should not only investigate the stress effects of high calcium soil environments on N. grossedentata but also assess the impacts of various stress conditions on the species.
Fig. 3.
Analysis of total calcium content of N. grossedentata on three soils. Different lowercase letters indicate significant differences (P<0.05). Error bars indicate standard error.
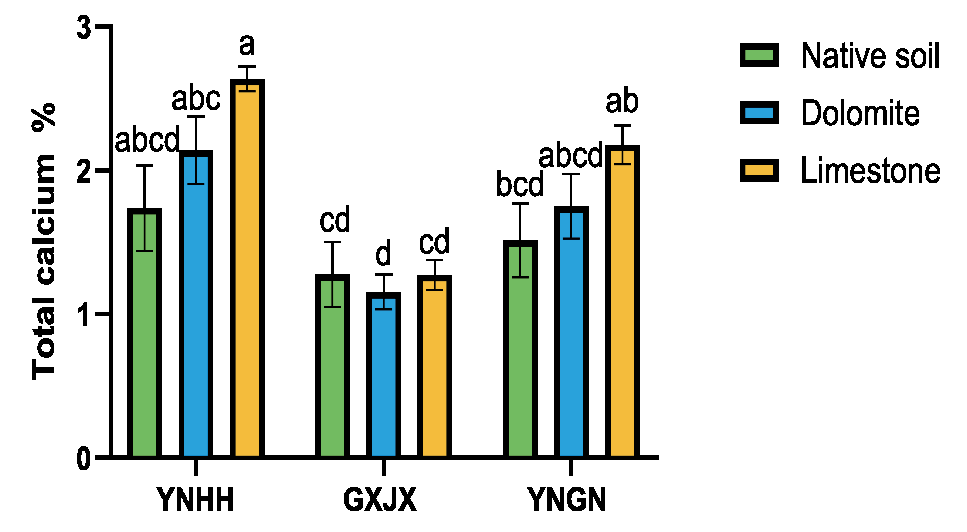
Fig. 4.
Correlation analysis between efficacy components, calcium content, and physiological and biochemical indexes of N. grossedentata. The correlation between nine physiological indicators is shown in the figure; the horizontal and vertical coordinates are nine different physiological indicators. Values in the table are the Pearson correlation coefficient. Close to 1 indicates a stronger positive correlation, close to –1 indicates a stronger negative correlation and close to 0 indicates no correlation. *P≤0.05; **P≤0.01 indicates extremely significant. TCL-Total calcium content of leaves; DMY-Dihydrosalicylate; TIN-Myricetin; TRIN-Myricetin; Chl-Chlorophyll; SS-Soluble sugar; TCS-Total calcium of soil; SCS-Soluble calcium of soil; PHS-PH of soil.
Conclusions
In conclusion, N. grossedentata demonstrates an ability to thrive in high-calcium environments, with key functional components such as dihydromyricetin generally increasing within karst soils, notwithstanding the variations in calcium absorption and effects observed across different genetic backgrounds. Chlorophyll and soluble sugars, which serve as indicators of stress resistance, exhibit significant changes under high-calcium conditions, suggesting that while the plant experiences a degree of stress, its survival is not compromised; rather, the production of functional substances is enhanced. This plant holds potential for use in the restoration of karst environments. Overall, it exhibits adaptability and tolerance to high-calcium settings, influencing the yield of its functional components. N. grossedentata’s adaptability and growth characteristics make it an ideal candidate for controlling rocky desertification. Its ability to rapidly establish vegetation cover, stabilize soils, and improve soil quality can help reverse desertification processes and restore ecosystem functionality in these degraded areas. While this study provides valuable insights into the physiological and biochemical responses of N. grossedentata to karst soil, it’s important to acknowledge its limitations: The study focused on three distinct genetic backgrounds (YNHH, GXJX, and YNGN). While this provides a comparative analysis, it doesn’t fully capture the genetic diversity within N. grossedentata. The future karst environment will have physiological and biochemical effects on more different genetic backgrounds of N. grossedentata, and it will be selected as the ideal N. grossedentata for repairing the karst stress environment.

