

Introduction
Diplandrorchis sinica, a saprophytic small herb of Dipladrorchis in Orchidaceae, is a unique monotypic orchid relict plant in China [1] and is a national Class II rare and endangered plant under protection [2]. The botanist Chen Xinqi (1979) discovered and proposed that Dipladrorchis is a very primitive and phylogenetically important new genus of Orchidaceae [2]. D. sinica is named for its two fertile stamens located in the apical ventral and dorsal direction of the stamen column. During the growth process, D. sinica may display flowers and no leaves. The plant has 13~17 pale green or greenish-white flowers. Petals are similar to labellum, anthers broadly ovate-oblong, stigma terminal, stamen beak absent, perianth nearly actinomorphic; the characteristics of nearly upright and rarely torsional flowers, upright stigma, and no stamen beak indicate that it should belong to the Bird nest orchid, one of the most primitive groups in Orchidaceae [3]. D. sinica lives saprophytic life. Years of investigation have found that it does not grow every year, and the number varies year to year, with a maximum of 14 plants found in one year. D. sinica is very demanding on the growing environment and has a short life cycle of only 15–20 days [4, 5]. Because the distribution area is extremely narrow, the population number of D. sinica is greatly limited. Therefore, how to save the small population and expand the population has become an urgent problem for orchid species conservation.
The germplasm resources of Chinese orchids are very rich, and the history of cultivation can be traced back to two thousand years ago [6]. Studies have shown that most orchids are rare and endangered species and have become the group of greatest concern in biodiversity conservation. In recent years, due to climate and environmental changes and the destruction of plant habitats, the number of endangered species of orchids has been decreasing, and the resources of orchids have been highly valued by researchers at home and abroad. At present, due to the limitation of the population and growth period of D. sinica, their pollination and reproduction methods are still unknown, which significantly restricts large-scale artificial breeding.
Soil microorganisms have been found to promote the growth and development of orchid roots, so the characteristics of their rhizosphere microbial community and rhizosphere ecological function have become hot spots for research at home and abroad. Studies have shown that orchids (Orchidaceae) are typical mycorrhizal plants, with small and large seeds without endosperm, which need to be symbiotic with suitable mycorrhizal fungi to germinate under natural conditions [7]. Seed germination, plant growth, and development of Cypripedium macranthum are closely related to mycorrhizal fungi. Isolated a strain of Epulorhiza sp from the fibrous roots of wild C. macranthum and confirmed that the fungus had a promotional effect on the seed germination of C. macranthum [8]. Most orchid plants grow in symbiosis with soil fungi [7, 8], and this mycorrhizal symbiosis accompanies almost the entire life history of orchids from seed germination to flowering and fruiting [6]. Endophytic fungi and bacteria in roots, stems, and other tissues of some orchid species play a very important role in their growth and development [9], seed germination [7, 10], and stress tolerance [6]. For example, Fusarium is a non-mycorrhizal fungus in the roots of orchid plants, which is effective in promoting the germination of orchid seeds, although it can induce plant diseases under certain conditions [11]. In one study, the dominant endophytic fungi of Euphorbiaceae were found to show a gradient of decreasing fungal abundance at three different horizontal distances from the root, inter-root soil, and root-enclosed soil during different reproductive growth periods, and its microhabitat fungal community was characterized by obvious seasonal changes in community structure and composition [12]. Inter-root microorganisms can coexist with the plant root system, colonize and sustain in the root system, and play an important role in promoting plant growth and development [13]. Among these microorganisms, the utilization and sensitivity of bacteria to root secretions is much higher than that of fungi, and bacteria are the most active and dominant microorganisms in the inter-root [14].
In recent years, the studies on D. sinica mainly focus on distribution area and phenological observation [15, 16], habitat characteristics [17], habitat investigation [18], and isolation of mycorrhizal fungi [19]. As a rare and endangered species of Orchidaceae, the study of rhizosphere and non-rhizosphere soil bacterial diversity of D. sinica has not been reported at home and abroad. Therefore, in order to characterize the bacterial community in the soil microorganisms of D. sinica, this study took rhizosphere and non-rhizosphere soil as the research object, and sequenced the V3~V4 region fragments of 16S rRNA gene of rhizosphere and non-rhizosphere soil bacteria based on Illumina Miseq high-throughput sequencing technology. The bacterial community structure and diversity characteristics of rhizosphere and non-rhizosphere soil of D. sinica were discussed at the molecular level, in order to provide scientific reference for the effective protection of endangered plant resources, and to lay a foundation for further discussion on artificial reproduction, habitat-mimicking cultivation and endangered mechanism of the D. sinica species.
Material and Methods
Soil Sample Collection
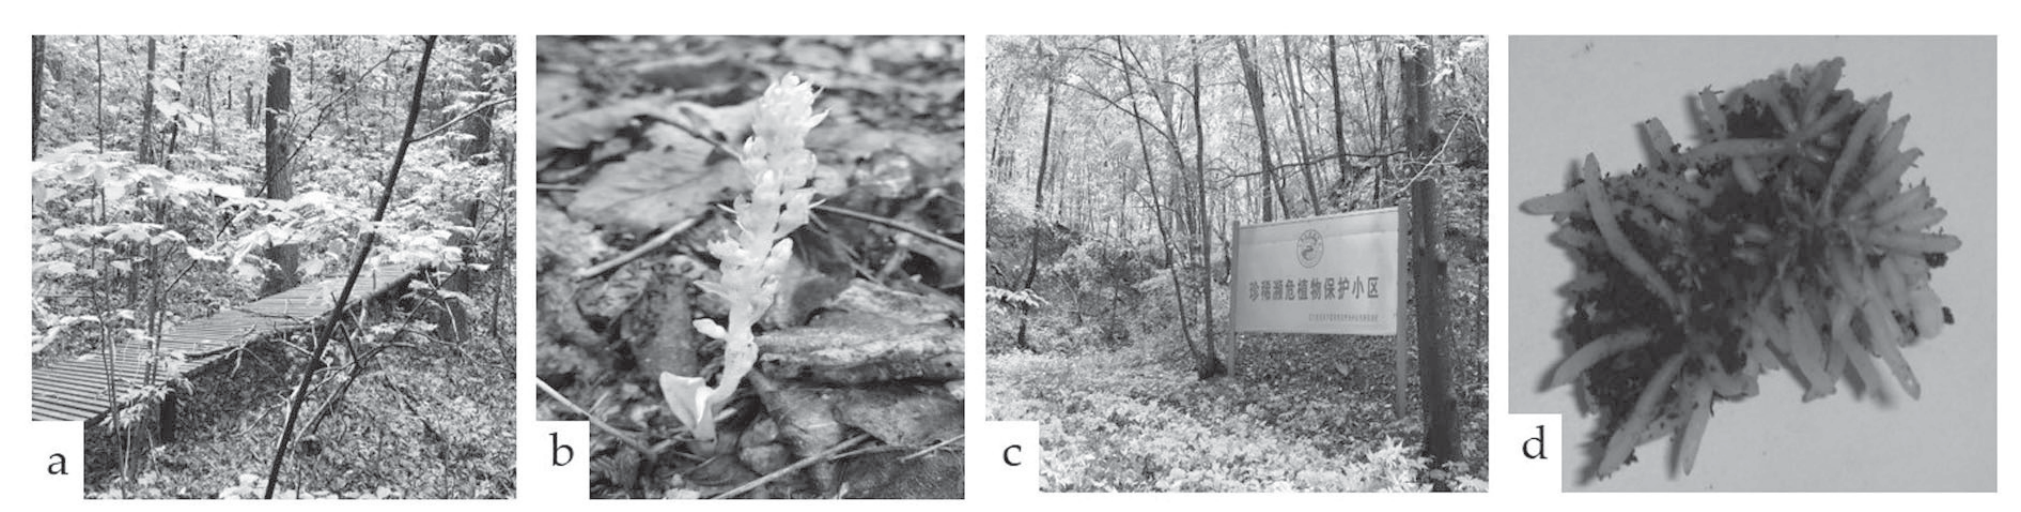
The growing site of D. sinica is located at Dadonggou Ranger Fire Station, Fushun Administration, Laohuadingzi Nature Reserve, Liaoning Province, 124°41’~125°05’E, 41°11’~41°21’N. The Rare and Endangered Conservation Area of Biruilan (Fig. 1-A) belongs to 2 subcompartments of 3 forest classes, and the survey area is 0.2 hectares. Acer mono, Quecus mongolica, Populus davidiana, Maackia amurensis, Juglans mandshurica, Tilia amurensis, Carpinus cordata, Amygdalus davidiana, Fraxinus rhynchophylla, Phellodendron amurense, Ulmus Rubra and other tree species grow in the reserve. The soil samples were collected from the Hongyan Forest Fire Station of Fushun Administration, Laotuding Nature Reserve, Liaoning Province (E124°41′13′′–125°5′15′′, N41°11′11′′–41°21′34′′) on August 10, 2016. In the habitat territory of D. sinica (Fig. 1-B) at an altitude of 632 m, soil with a depth of 0~20 cm was taken from the root zone of D. sinica (Fig. 1-C), the large soil chunks attached to the fleshy roots were shaken off, and then the rhizosphere soil attached to the fleshy roots was collected with small tweezers (Fig. 1-D). The soil was collected as rhizosphere soil, and 4 replicates were labeled as T1, T2, T3, and T4, respectively. At the same time, 10 collection sites were randomly set along the S-shaped path in its protection area, and the surface soil was removed. The sterilized ring knife was used to collect the soil at each collection site, and the soil was mixed and put into the sterilized encapsulation bag, which was labeled as non-rhizosphere soil samples. The four repeated sites were labeled as T5, T6, T7, and T8. Soil samples were placed in sterile sealed plastic bags, placed in ice boxes, and brought back to the laboratory. Some soil samples were naturally air-dried, ground and screened indoors, and stored in a refrigerator at 4°C for the determination of basic physical and chemical properties of soil. The other part of the samples were stored in the refrigerator at -80°C for soil microbial index analysis.
Determination of Soil Physical and Chemical Properties
The samples from rhizosphere and non rhizosphere soils of D. sinica were used for physicochemical properties determination. The soil pH was measured using a pH meter. Total nitrogen (TN) was measured using the Kjeldahl method, in which the TN in soil samples was converted into NH3 by boiling with concentrated H2SO4 and the catalytic agent, and then distilling with NaOH. The NH3 was evaporated into a boric acid indicator and then titrated using a standard solution of HCl. Hydrolyzed nitrogen (HN) was measured using the alkaline hydrolysis diffusion method, in which the soil samples were hydrolyzed with NaOH solution in a sealed diffusion dish, and the HN was converted into NH3 and constantly spread and escaped. The NH3 was absorbed by the boric acid indicator and then titrated using a standard solution of HCL, the same as described above.
Total potassium (TK) and fast-acting potassium (AK) were measured using the flame photometric method. TK was determined using the melting method with NaOH in a silver crucible, in which the TK was converted into soluble potassium and then the TK concentration in the solution was determined by referring to the potassium standard curve after being measured using a flame photometer. The AK was determined by CH3COOK immersion extraction. The soil samples were added into a 10-fold volume of CH3COOK and then the extracted solutions were used for AK concentration determination, the same as described above.
Total phosphorus (TP) and available phosphorus (AP) were measured by the molybdenum blue colorimetric method. Total phosphorus extraction is the same as total potassium, which converts the total phosphorus into soluble phosphorus and then adds dinitrophenol indicator and molybdenum antimony antichromogen. The solution was used for TP concentration determination by referring to the phosphorus standard curve after being measured using a spectrophotometer. The phosphorus standard curve was drawn by the concentrations of the standard phosphorus solution that reacted with the molybdenum antimony antichromogen and their absorption value. AP was extracted by NaHCO3 immersion extraction, of which the available phosphorus in soil samples was dissolved in NaHCO3. The available phosphorus concentration in the solution was determined as the same as above. The total phosphorus and available phosphorus contents were then calculated.
The soil organic carbon (SOC) was measured by the potassium dichromate (K2Cr2O7) external heating method. The SOC in the soil samples was converted into CO2 after boiling in a K2Cr2O7 solution, and the dichromate ion was reduced to a trivalent chromium ion. The remaining K2Cr2O7 was titrated with the FeSO4 standard solution, and then the SOC content was calculated according to the difference between the used FeSO4 for soil samples and the blank control. Soil organic matter (SOM) content was calculated as 1.724 × SOC, and the carbon-nitrogen ratio in soil organic matter was calculated as SOC/ TN.
Extraction of Total DNA from Soil Genome
DNA extraction was extracted using MO BIO Power Soil DNA Extraction Kit (MO BIO Laboratories, Carlsbad, CA, USA). DNA concentration and quality were checked using a NanoDrop Spectrophotometer. Extracted DNA was diluted to 10 ng/μL and stored at -40°C for downstream use.
PCR Amplification
Universal primer for bacteria 16S: F515: 5’- GTGC- CAGCMGCCGCGG-3’ and R909: 5’-CCCCGYCAATTC- MTTTRAGT-3’with 12 nt unique barcode was used to amplify the V4 hypervariable region of 16S rRNA gene for pyrosequencing using Miseq sequencer [20, 21]. The PCR mixture (25uL) contained 1x PCR buffer, 1.5 mM MgCl2, each deoxynucleoside triphosphate at 0.4 uM, each primer at 1.0uM and 0.5U of ExTaq (TaKaRa, Dalian) and 10ng soil genomic DNA. The PCR amplification program included initial denaturation at 94°C for 3 min, followed by 30 cycles of 94°C for 40 s, 56°C for 60 s, and 72°C for 60 s, and a final extension at 72°C for 10 min. Conduct two PCR reactions for each sample, and combine them together after PCR amplification. PCR products were subjected to electrophoresis using 1.0% agarose gel. The band with the correct size was excised and purified using SanPrep DNA Gel Extraction Kit (Sangon Biotech, China, Cat# SK8132) and quantified with Nanodrop. All samples were pooled together with an equal molar amount from each sample. The sequencing samples were prepared using a TruSeq DNA kit according to the manufacturer’s instructions. The purified library was diluted, denatured, re-diluted, mixed with PhiX (equal to 30% of the final DNA amount) as described in the Illumina library preparation protocols, and then applied to an Illumina Miseq system for sequencing with the Reagent Kit v2 2×250 bp as described in the manufacture manual.
Data Analysis
The sequence data were processed using QIIME Pipeline-Version 1.7.0 (http://qiime.org/). All sequence reads were trimmed and assigned to each sample based on their barcodes. The sequences with high quality (length > 150 bp, without ambiguous base ‘N’, and average base quality score > 30) were used for downstream analysis. Sequences were clustered into operational taxonomic units (OTUs) at a 97% identity threshold. The aligned ITS gene sequences were used for chimera check using the Uchime algorithm [22]. All the samples were randomly resampled to 28,894 reads. We calculated alpha-diversity (phylogenetic distance whole tree, chao1 estimator of richness, observed species, and Shannon’s diversity index) and beta-diversity (PCoA, UniFrac) analyses, for which the rarefaction curves were generated from the observed species. Taxonomy was assigned using the Ribosomal Database Project classifier [23].
Results
Determination of Physical and Chemical Properties of Soil in D. Sinica Habitat
From Table 1, we can see that the pH of the rhizosphere soil of D. sinica is higher than that of the non-rhizosphere soil, but there is no significant difference between the two, which is a neutral acidic soil; the contents of total nitrogen (TN), total potassium (TK), total phosphorus (TP), available phosphorus (AP), soil organic matter (SOM), hydrolyzed nitrogen (HN) and fast-acting potassium (AK) in the rhizosphere soil are significantly higher than that of the non-rhizosphere soil (p < 0.01); while the soil organic carbon (SOC) and soil carbon to nitrogen ratio of the rhizosphere soil are lower than that of the non-rhizosphere soil (p < 0.01). These results indicate that the growth of D. sinica requires a high SOM, HN, and AK, and neutral to acidic pH.
Bacterial Alpha Diversity in Rhizosphere and Non-Rhizosphere Soil of D. sinica
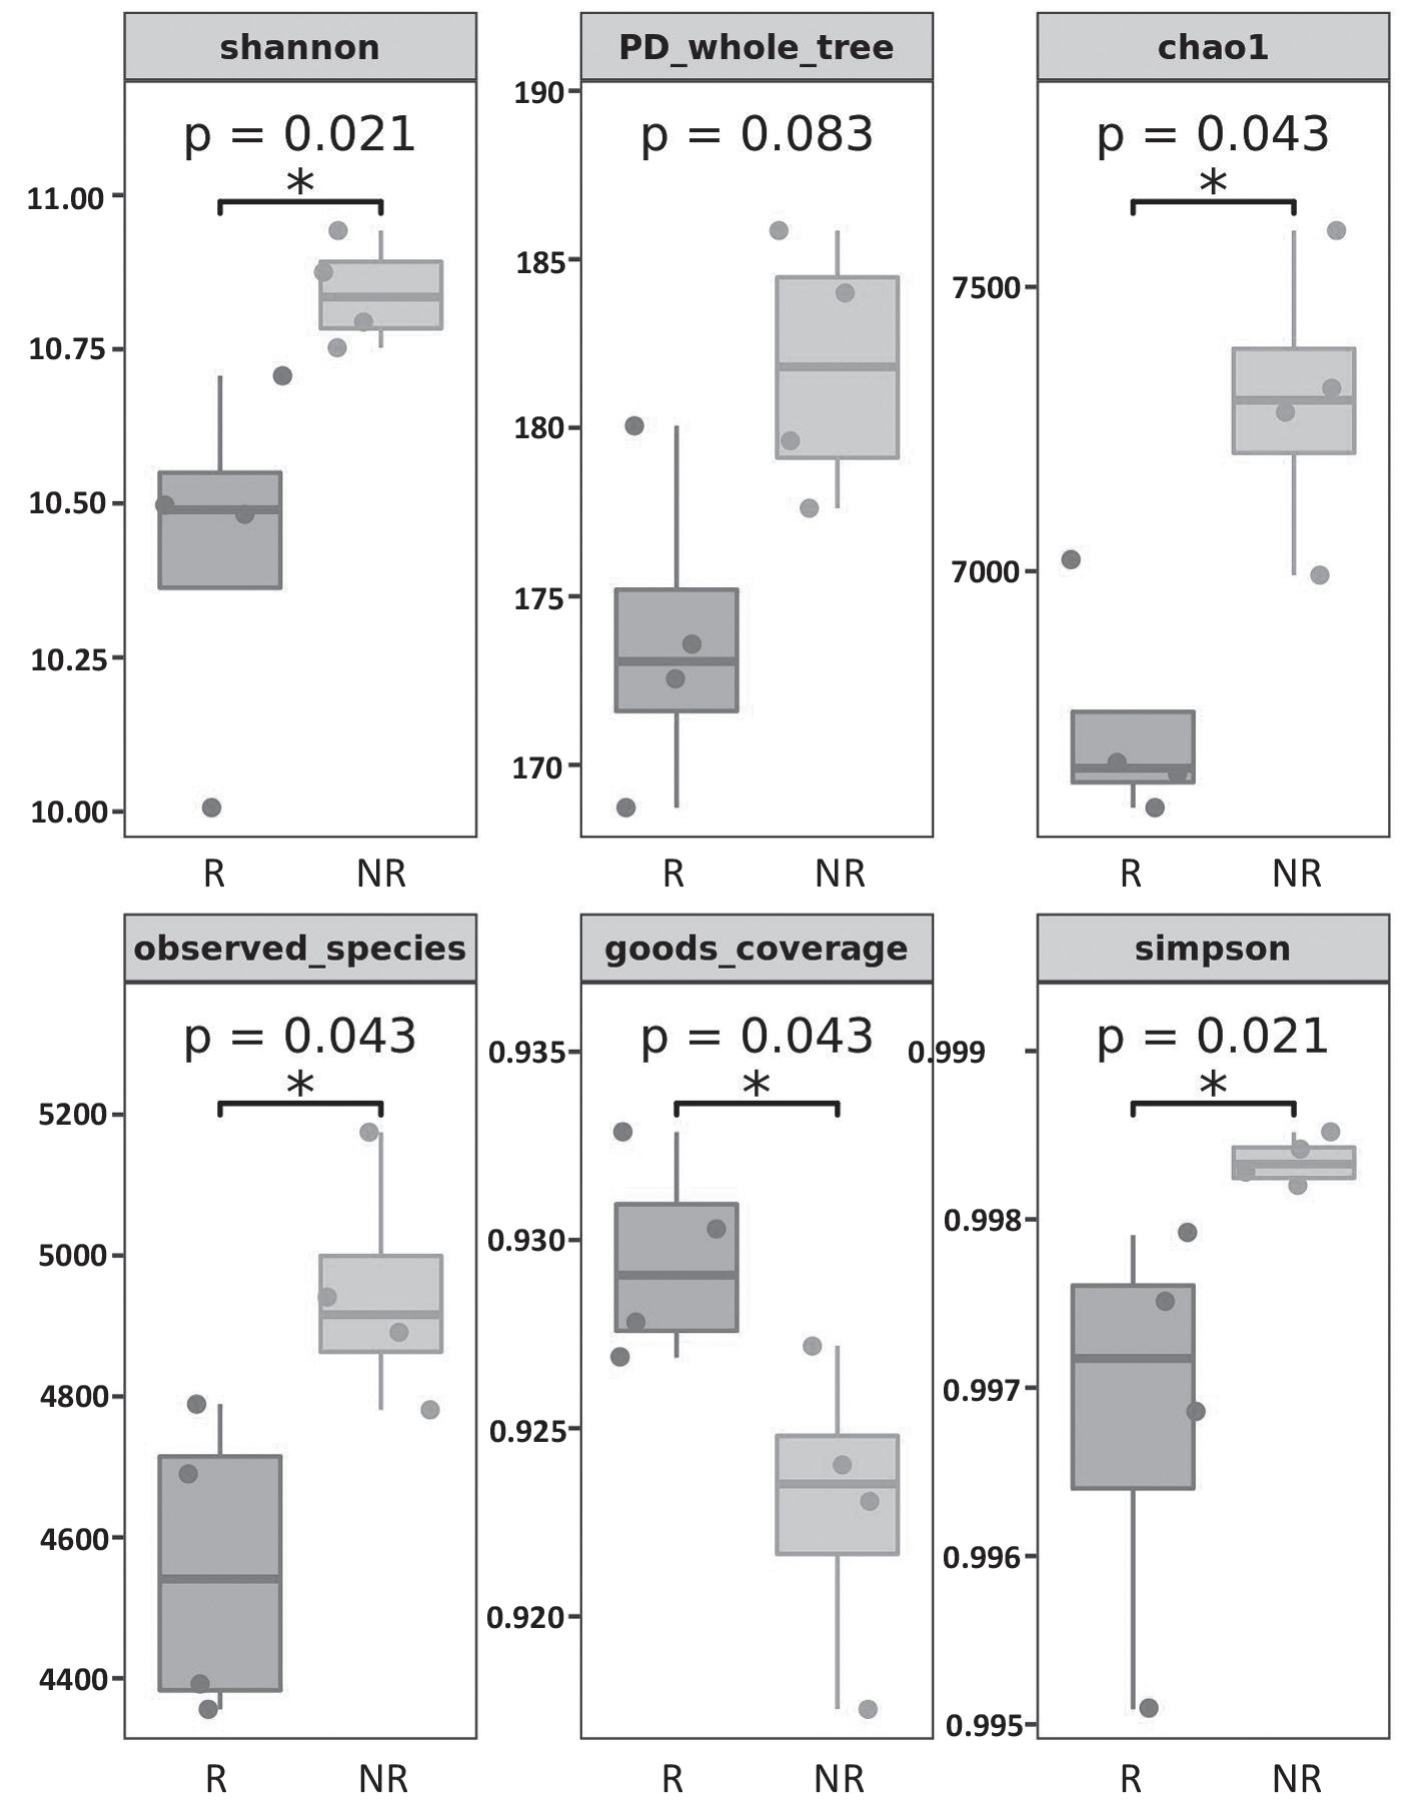
High-throughput sequencing of 16S rRNA V3-V4 regions of rhizosphere and non-rhizosphere soil bacteria of D. sinica was performed, and a total of 26,690 raw sequences were obtained from high-throughput sequencing of bacterial 16S rRNA genes. 26,471 valid sequences were obtained after splicing and filtering, and 9,556 OTUs belonging to 34 phyla, 113 orders, 361 families, and 551 genera were classified after clustering analysis. The Shannon index and Chao1 index of the bacterial community in rhizosphere soil were 10.42 and 6728.07, respectively, while the Shannon index and Chao1 index of the non-rhizosphere soil were 10.84 and 7298.39, respectively. It can be seen from Fig. 2 that the Shannon, Chao1, and Simpson indices of the rhizosphere soil were lower than those of the non-rhizosphere soil, with significant differences (p <0.05).
Table 1.
Analysis of physicochemical properties of rhizosphere and non-rhizosphere root soils of Diplandrorchis sinica.
Analysis of Bacterial Community Composition and Abundance in Rhizosphere and Non-Rhizosphere Soils of D. sinica
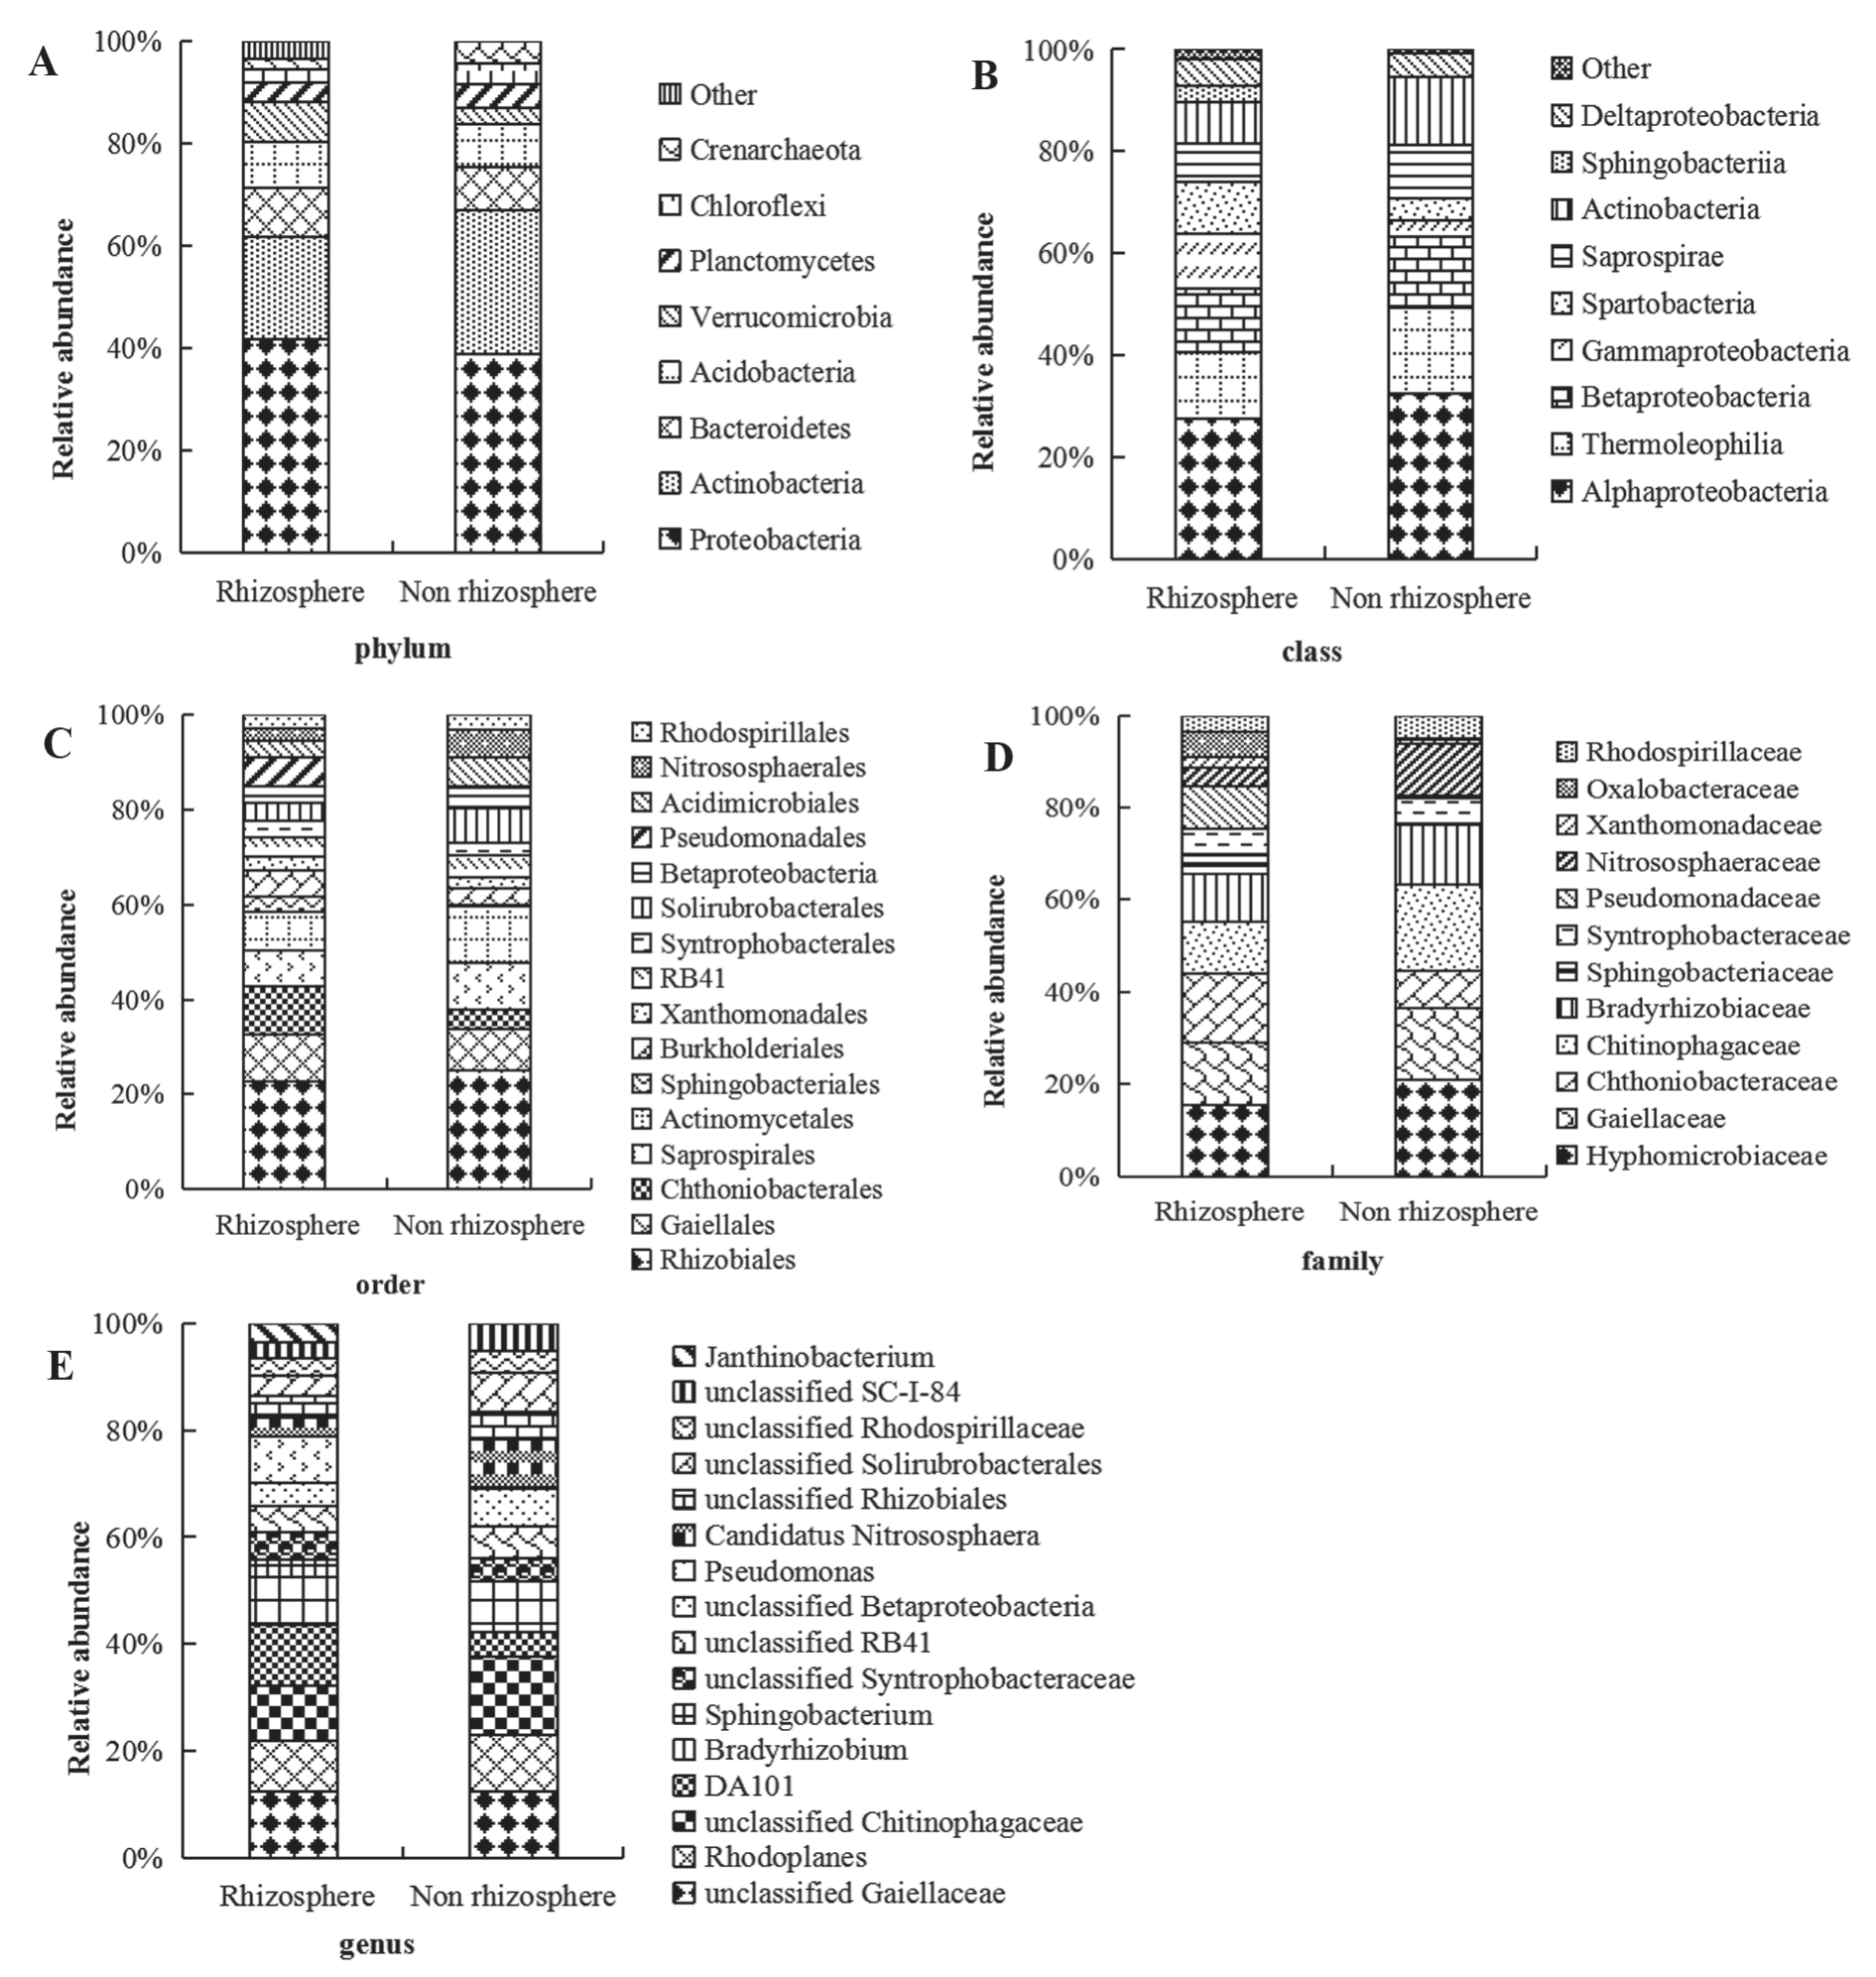
After filtering the original sequences and counting the number of each species in each sample, a statistical table of species of rhizosphere and non-rhizosphere soil bacteria of D. sinica can be obtained. There are no significant differences in the numbers of phylum, class, order, family, and genus between rhizosphere and non-rhizosphere soil of D. sinica, and most of the phylum, class, order, family, and genus are common both in rhizosphere and non-rhizosphere soil (Table 2).
At the phylum taxonomic level (Fig. 3-A), Proteobacteria dominated the rhizosphere and non-rhizosphere soil bacterial taxa of D. sinica, accounting for 41.87% and 37.97% (p > 0.05), respectively, followed by Actinbacteria, accounting for 19.93% and 27.45% (p < 0.01), respectively, Bacteroidetes, accounting for 9.57% and 8.11% (p > 0.05), respectively, and Acidobacteria, accounting for 9.01% and 8.11% (p < 0.05), respectively, Verrucomicrobia (7.67% and 3.23%, p < 0.05), and Planctomycetes (3.81% and 4.40%, p > 0.05), respectively.
At the level of bacterial class (Fig. 3-B), the dominant bacterial taxa in the rhizosphere and non-rhizosphere soils of D. sinica were mainly α-Alphaproteobacteria (20.39% and 22.55%, p > 0.05), Thermoleophilia (9.76% and 11.61%, p > 0.05), β-Alphaproteobacteria (9.27% and 9.67%, p > 0.05), Gammaproteobacteria (8.13% and 2.36%, p > 0.05), Spartobacteria (7.43% and 2.99%, p < 0.05), Saprospirae (5.67% and 7.14%, p > 0.05) and Actinobacteria (5.99% and 9.26%, p < 0.01).
At the level of bacterial orders (Fig. 3-C), the dominant bacterial taxa in the rhizosphere and non-rhizosphere soil of D. sinica were mainly Rhizobiales (16.68% and 18.22%, p > 0.05), Gaiellales (7.01% and 6.45%, p > 0.05), Chthoniobacterales (7.43% and 2.99%, p < 0.05), Saprospirales (5.67% and 7.14%, p > 0.05), and Actinomycetales (5.84% and 8.91%, p < 0.05), Sphingobacteriales (2.35% and 0.16%, p < 0.05), Burkholderiales (4.11% and 2.59%, p > 0.05), Xanthomonadales (2.11% and 1.70%, p > 0.05), RB41 (2.88% and 3.22%, p < 0.05), Syntrophobacterales (2.65% and 2.11%, p < 0.05), Solirubrobacterales (2.75% and 5.14%, p < 0.05).
At the bacterial family level (Fig. 3-D), the main dominant bacteria in the rhizosphere and non-rhizosphere soil of D. sinica were: Hyphomicrobiaceae (7.62% and 7.87%, p > 0.05), Gaiellaceae (6.72% and 5.96%, p > 0.05), Chthoniobacteraceae (7.43% and 2.99%, p < 0.05), Chitinophagaceae (5.62% and 7.09%, p > 0.05), Bradyrhizobiaceae (5.11% and 4.97%, p > 0.05), Sphingobacteriaceae (2.22% and 0.06%, p < 0.05), Syntrophobacteraceae (2.65% and 2.11%, p > 0.05), Pseudomonadaceae (4.63% and 0.14%, p < 0.05), Nitrososphaeraceae (1.90% and 4.27%, p < 0.05), Xanthomonadaceae (1.24% and 0.39%, p < 0.05), Oxalobacteraceae (2.67% and 0.06%, p < 0.05) and Rhodospirillaceae (1.80% and 1.92%, p > 0.05).
At the bacterial genus level (Fig. 3-E), the main dominant bacteria in the rhizosphere and non-rhizosphere soil of D. sinica were: Rhodoplanes (5.08% and 5.04%, p > 0.05), DA101 (6.20% and 2.23%, p > 0.05), Bradyrhizobium (4.69% and 4.44%, p > 0.05), Sphingobacterium (1.85% and 0.001%, p < 0.05), Pseudomonas (4.62% and 0.14%, p < 0.05) and Candidatus Nitrososphaera (1.89% and 4.26%, p > 0.05), respectively. In addition, there are some unclassified Gaiellaceae, unclassified Chitinophagaceae, unclassified Syntrophobacteraceae, unclassified RB41, β-Amorphic (unclassified Betaproteobacteria), Rhizobiales (unclassified Rhizobia), Solirubrobacterales (unclassified Solirubrobacterales), and Rhodospirillaceae (unclassified Rhodospirillaceae), together accounting for 25.89% and 28.90%, respectively.
Relationship Between the Dominant Bacterial Taxa and Soil Physicochemical Properties in D. sinica Habitats
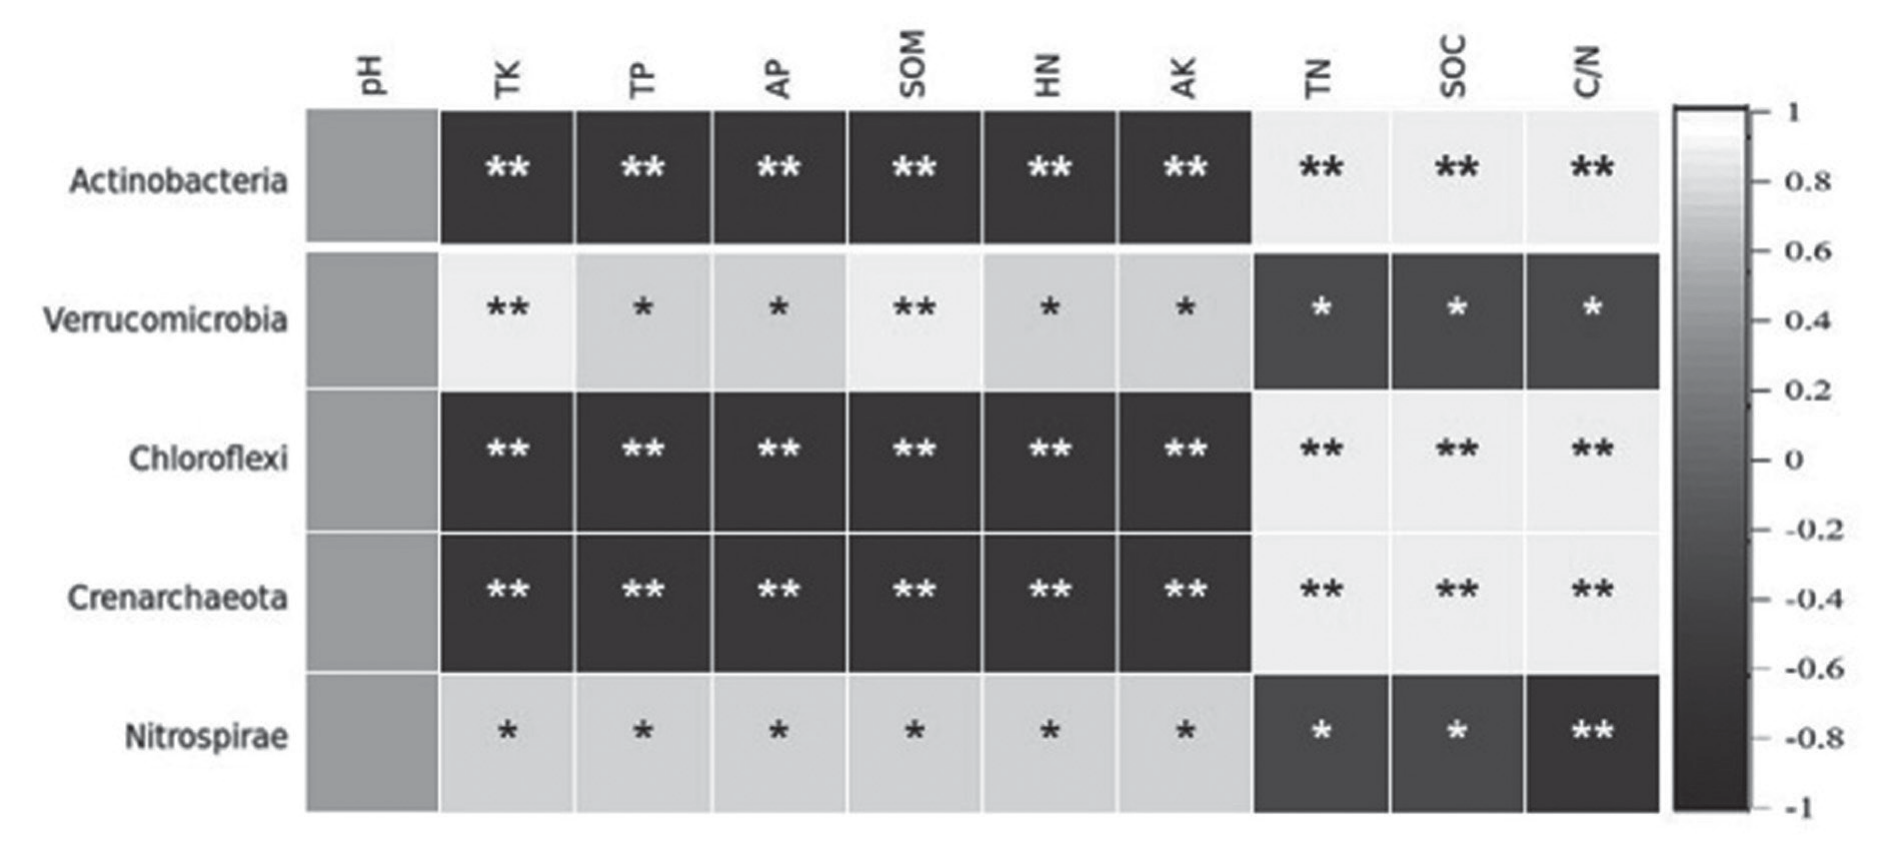
The redundancy analysis of rhizosphere and non-rhizosphere soil microorganisms and their soil physicochemical properties of D. sinica was performed, and the results can be seen in Fig. 4: for the two axes of the soil bacterial community RDA contributions were 68.66% and 24.28%, respectively, and the four samples of rhizosphere soil of D. sinica were clustered on one side, but T1, T2, T4, and T3 were far away from each other, indicating differences between samples, while the four samples of non-rhizosphere soil were clustered together. A total of 92% of the total characteristic values were explained by the five selected basic soil physicochemical properties, in which soil values of available phosphorus (AP), hydrolyzed nitrogen (HN), total phosphorus (TP), total potassium (TK), and pH of rhizosphere soils were significantly different from those of non-rhizosphere soils. Soil microorganisms of the phylum Proteobacteria, Actinobacteria, and Verrucomicrobia were significantly and positively correlated with each other and influenced the rhizosphere soil microbial abundance of D. sinica. Specifically, Actinobacteria, Chloroflexi, and Crenarchaeota were highly significantly negatively correlated with soil TK, TP, AP, soil organic matter content (SOM), HN, AK, and highly significantly positively correlated with TN, SOC (Soil organic carbon), and C/N (p < 0.01) (Fig. 5). The Verrucomicrobia showed highly significant positive correlations with TK and SOM content (p < 0.01), significant positive correlations with TP, AP, HN, AK (p < 0.05), and significant negative correlations with TN, SOC, and C/N (p < 0.05). Nitrospirae showed significant positive correlations with soil TK, TP, AP, SOM, HN, and AK (p < 0.05), significant negative correlation with TN and SOC (p < 0.05), and highly significant positive correlation with soil C/N (p < 0.01, Fig. 5).
Fig. 4.
RDA redundancy analysis of dominant rhizosphere (R) and non-rhizosphere (NR) bacteria and soil physical and chemical properties. T1-T4 represented the 4 duplicates of rhizosphere soil samples, and T5-T8 represented the 4 duplicates of non-rhizosphere soil samples. pH, potential of hydrogen; TN, total nitrogen; TK, total potassium; TP, total phosphorus; AP, available phosphorus; HN, hydrolyzed nitrogen.
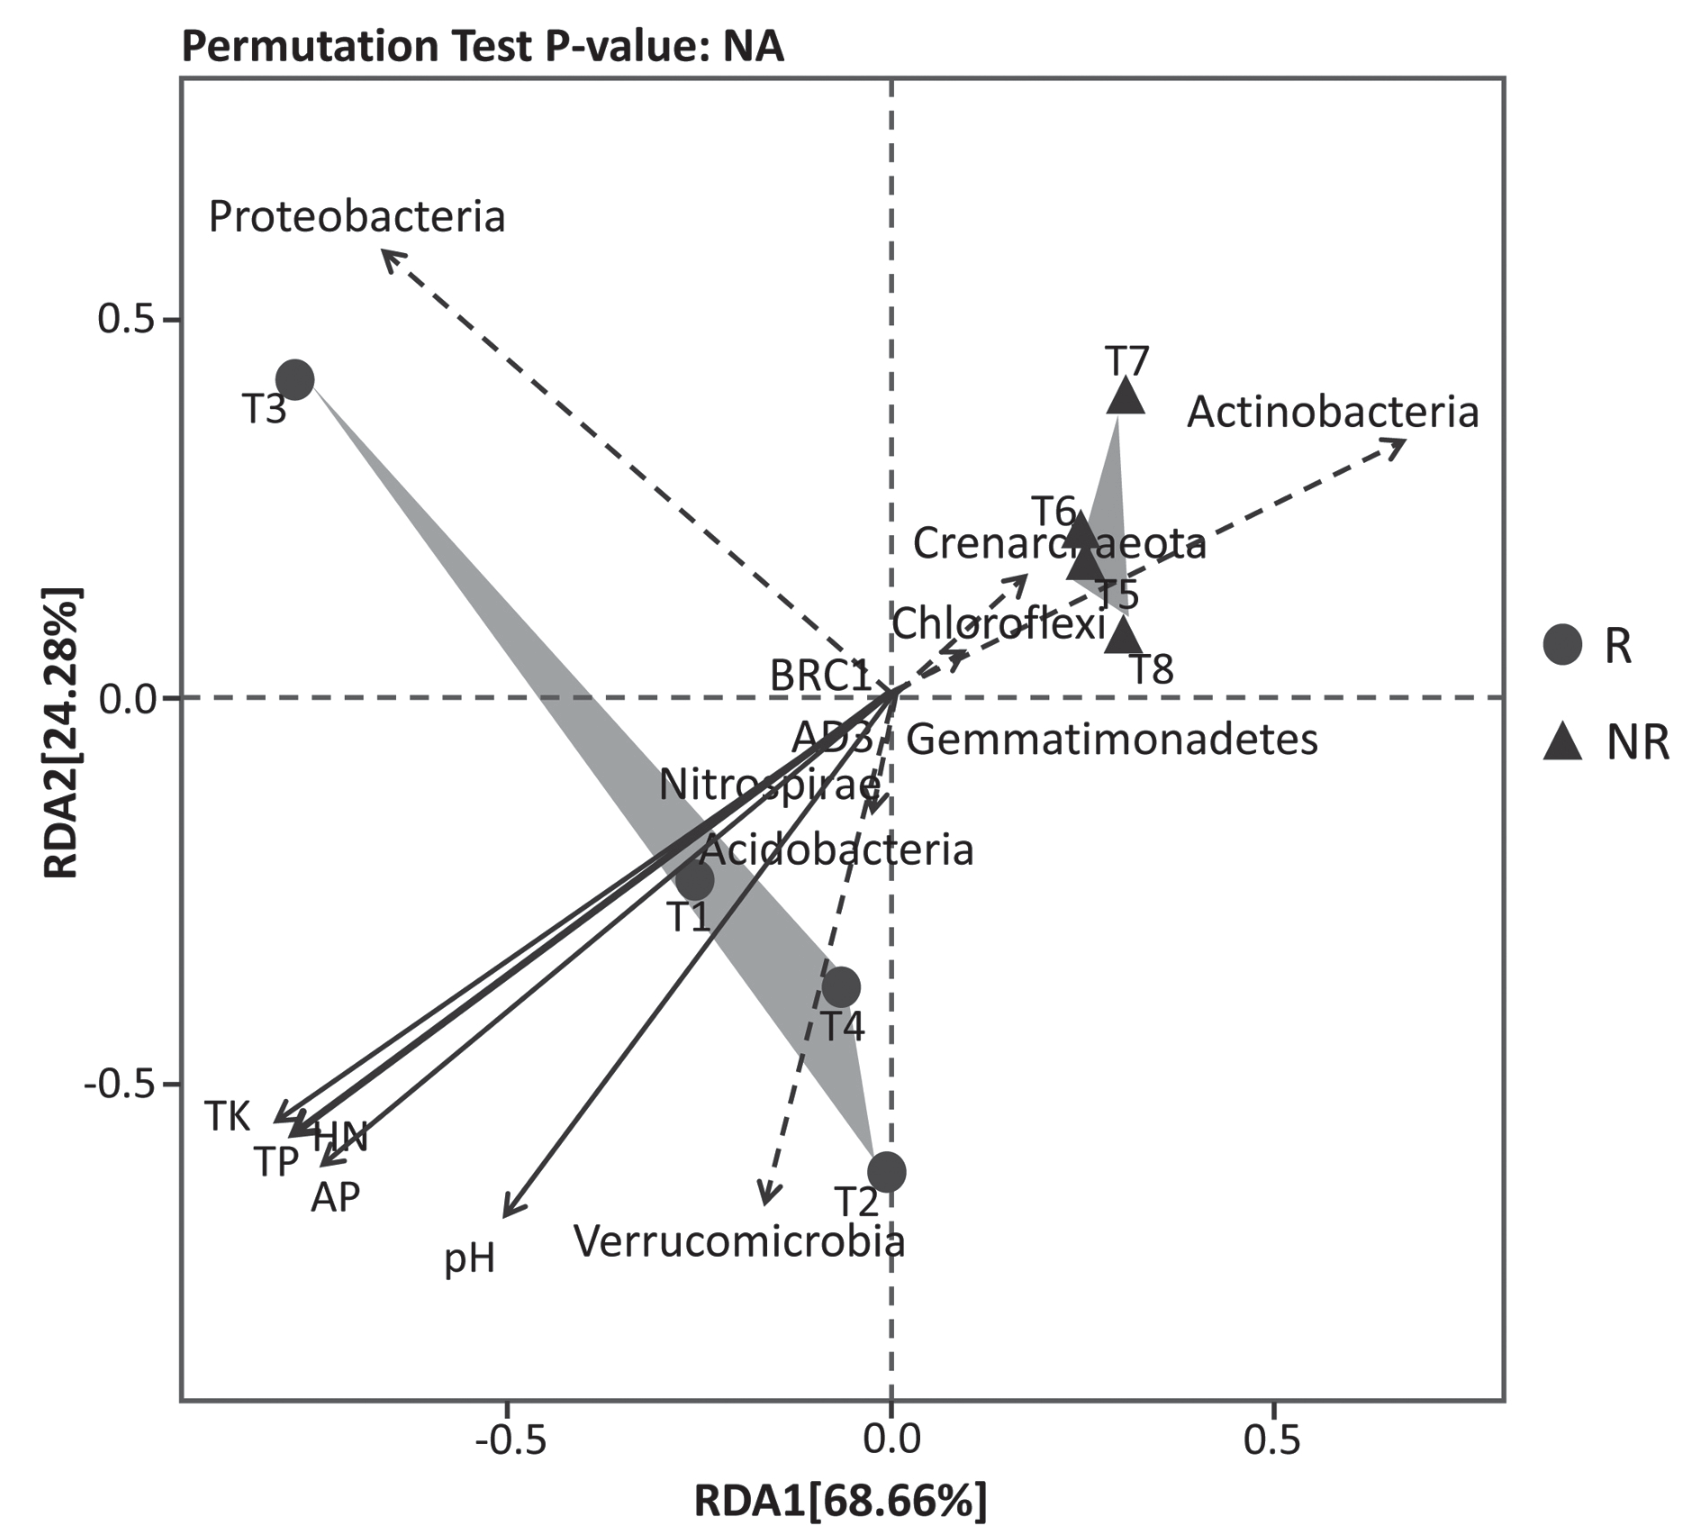
Fig. 5.
Correlation analysis between dominant bacterial phyla groups and soil physical and chemical properties. pH, potential of hydrogen; TK, total potassium; TP, total phosphorus; AP, available phosphorus; SOM, soil organic matter; HN, hydrolyzed nitrogen; AK, fastacting potassium; TN, total nitrogen; SOC, Soil organic carbon; C/N, Carbon to nitrogen ratio.
Microbial Markers of Rhizosphere and Non-Rhizosphererhizal Soil Bacteria in D. sinica
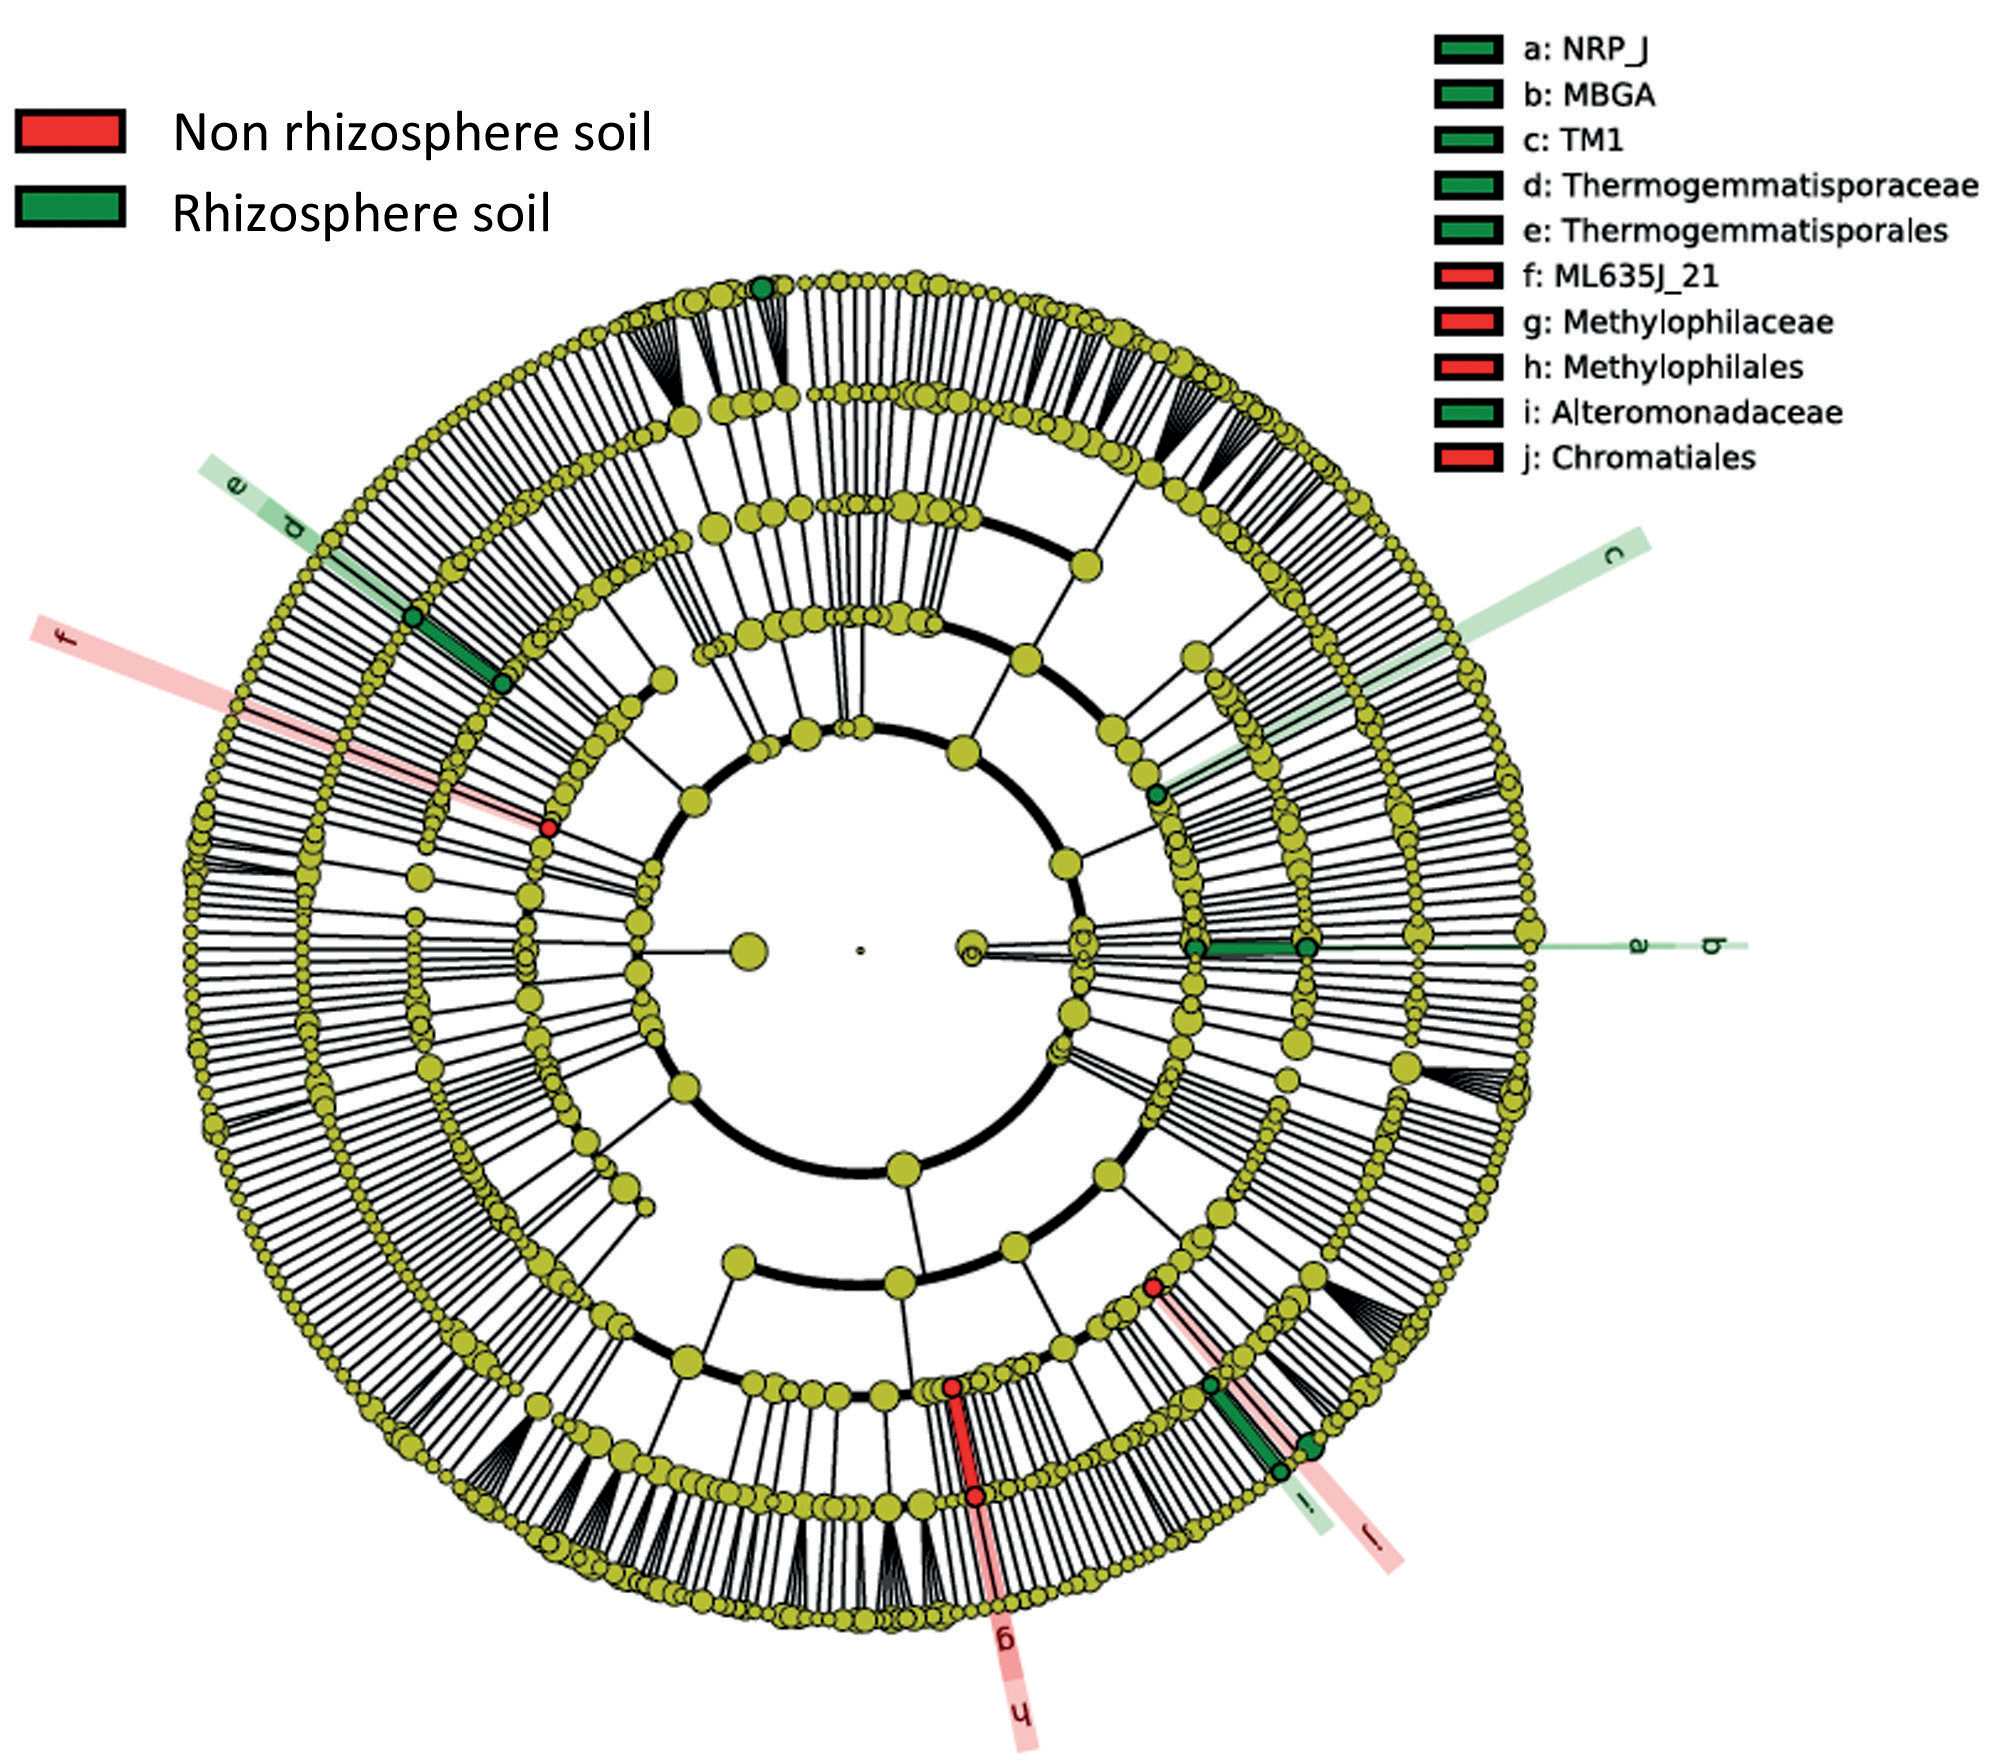
The classification level of the tree diagram in Fig. 6 proceeds from the phylum to the genus. Node size indicates the relative abundance of each sample grouping. Nodes of different colors indicate significantly enriched microorganisms in the corresponding groups, which had a significant effect on the differences between groups, while yellow nodes indicate that microorganisms were not significantly different in any of the different groups.
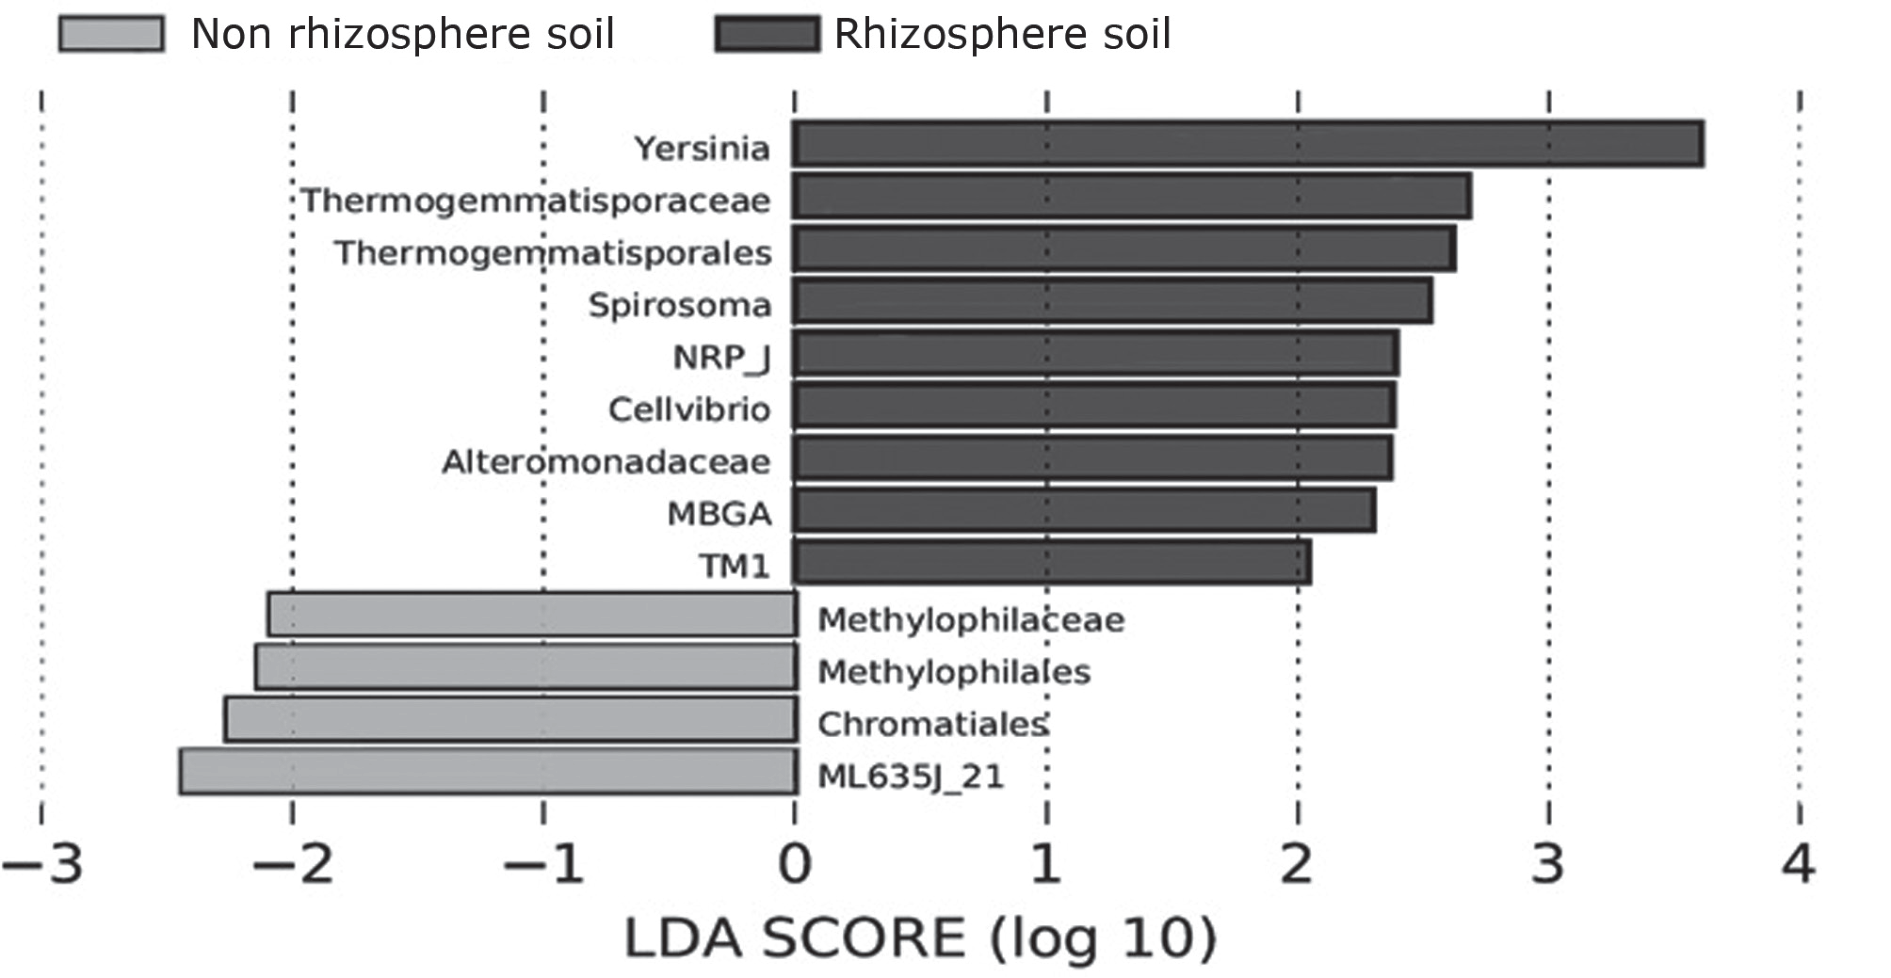
LEfSe was used to analyze the rhizosphere and non-rhizosphere soil microorganisms of D. sinica separately to find the indicator species for each treatment. Linear discriminant analysis (LDA) was performed on samples according to different grouping conditions to identify bacteria that had a significant differential effect on sample delineation. The results showed that rhizosphere soil bacterial microbial diversity was rich, with significant differences (p < 0.05) between rhizosphere and non-rhizosphere soil bacterial microorganisms (as in Fig. 5); when LDA > 2, p < 0.05, the main rhizosphere soil bacterial biomarkers of D. sinica were Yersinia, Thermogemmatisporales, Spirosoma, NRP_I, Cellvibrio, Alteromonadaceae, MBGA and TM1; non-rhizosphere soil bacterial biomarkers are mainly Methylophilaceae, Methylophilales, Chromatiales, and ML635J_21 (e.g., Fig. 7).
Discussion
The pH of the rhizosphere soil of the endangered species of D. sinica was slightly higher than the pH of the non-rhizosphere soil, which may be due to the secretion produced by the fleshy roots of D. sinica into the rhizosphere soil, thus causing the high pH of the rhizosphere soil. The contents of total nitrogen, total potassium, total phosphorus, available phosphorus, soil organic matter content, hydrolyzed nitrogen, and available potassium in the rhizosphere soil of D. sinica were significantly higher than those in the non-rhizosphere soil (p < 0.05), while the contents of total nitrogen, soil organic carbon, and soil carbon to nitrogen ratio in the rhizosphere soil of D. sinica were lower than those in the non-rhizosphere soil, and the differences between them were highly significant (p < 0.01). This indicates that the growth of D. sinica can increase the rhizosphere soil pH, and the organic matter secreted by the rhizosphere during the growth process, enters the rhizosphere soil, which leads to the difference between the rhizosphere soil and non-rhizosphere soil in terms of physicochemical properties. This phenomenon of nutrient enrichment in the soil in the rhizosphere region occurs in Solidago canadensis, Larix principis-rupprechtii, Paris polyphylla, and Choerospondias axillaris among other species are consistent with the findings [24–27].
Soil microorganisms are important components of soil, the analysis of soil Illumina Miseq of the rare and endangered plant indicated that the dominant taxa of rhizosphere and non-rhizosphere soil bacteria of D. sinica were mainly Proteobacteria, Alphaproteobacteria, Rhizobiales, Hyphomicrobiaceae, and unclassified Gaiellaceae genus. However, the inter-rhizosphere soil microbial bacterial α-diversity in D. sinica was lower than in non-rhizosphere soils, and the two were significantly different (p < 0.05), and this finding is consistent with the study of inter-rhizosphere microorganisms of the endangered plant Cypripedium macranthos [28]. Similar results were also reported in the research about the soil bacterial community structure diversity in vineyards [29] and the natural secondary forest soil microbial community characteristics of Quercus mongolica [30]. Currently, Sphingosine bacteria and Branchomycetes have been isolated from the roots of Dendrobium moschatum, and these two strains of bacteria were inoculated with D. moschatum seeds, and the results showed that the species could promote seed germination [28]. Many domestic scholars have also identified Pseudomonas and Bacillus as the dominant orchid species from endophytic bacterial isolation of orchid species such as Cymbidium, Dendrobium, and Goodyera [31–33].
Soil inter-rhizosphere is a special ecosystem with significant differences in chemical and biological properties between rhizosphere and non-rhizosphere soils. Rhizosphere soil is susceptible to plant roots and is a tiny area where complex interactions between beneficial and harmful microorganisms and host plants occur. Root secretions and the microenvironment also influence soil physical and chemical properties and soil microbial community distribution [34, 35]. Therefore, plant roots, soil environment, and soil microorganisms interact with each other to form a stable and reciprocal relationship that promotes plant growth and development [36–37]. Plants also have active selectivity on the rhizosphere soil bacterial community structure [38]. Plants change the inter-root environment through root activities, thus selectively increasing or decreasing the abundance or diversity of certain rhizosphere soil bacterial taxa, so that the abundance of bacterial species beneficial to the plant’s own growth increases, while bacterial species unfavorable to its own growth decreases or even disappears, thus forming an inter-root bacterial community structure beneficial to itself. This results in different plants having different rhizosphere bacterial composition structures [39]. The results of this study revealed that soil values of total nitrogen (TN), active phosphorus (AP), hydrolyzed nitrogen (HN), total phosphorus (TP), total potassium (TK), and pH in the rhizosphere soil of D. sinica were significantly different from those of non-rhizosphere soil; and were significantly correlated with soil microorganisms of Proteobacteria, Actinobacteria, and Verrucomicrobia. These dominant groups influence the abundance of microbial bacteria in the rhizosphere soil of D. sinica. Bradyrhizobium, Sphingobacterium, and Pseudomonas are the main genera in the rhizosphere soil of D. sinica, which play important roles in increasing the organic matter content in the rhizosphere soil [40], promoting nitrogen fixation by rhizosphere microorganisms [41] and suppressing fungal diseases [42]. Meanwhile, we used LEfSe analysis in order to explore the indicator species among soil microbial bacteria affecting the endangerment of P. bifidum, and found that hundreds of indicator species could be found when the alpha level was 0.05 (catalog lefse 0.05), but no indicator species could be found when the alpha level was 0.01, so we chose 13 indicator species at the condition of LDA > 2, p < 0.05, of which the main inter-rhizosphere soil bacterial biomarkers of D. sinica were Yersinia, Thermogemmatisporaceae, Thermogemmatisporales, Spirosoma, NRP_I, Cellvibrio, Alteromonadaceae, MBGA, and TM1, indicating that the fleshy roots of D. sinica are significantly enriched for these groups during growth; while the non-rhizosphere soil bacterial biomarkers are mainly Methylophilaceae, Methylophilales, Chromatiales and ML635J_21.
The discovery of these indicator species has laid the foundation for the study of the endangerment mechanism of D. sinica. In addition, from the analysis of the high-throughput sequencing results of the rhizosphere and non-rhizosphere soils in this study, there is still a large number of unidentified groups of soil bacteria in the inter-rhizosphere soil of D. sinica, among which the key bacteria affecting the endangerment of D. sinica may be unearthed, which will be analyzed in depth in the next step.
Conclusions
In this study, we analyzed the physical and chemical properties and microbial community characteristics of rhizosphere and non-rhizosphere soil in the D. sinica population. The results showed a significant difference in total nitrogen (TN), available phosphorus (AP), hydrolyzed nitrogen (HN), total phosphorus (TP), total potassium (TK), and pH in rhizosphere and non-rhizosphere soil of the D. sinica population. The soil physical and chemical properties affected the microbial and bacterial richness in rhizosphere soil of the D. sinica population. Soil bacterial diversity is rich, with the main dominant bacteria Proteobacteria, Bacteroidetes, Acidobacteria, and Verrucomicrobia at the phylum level; α-Alphaproteobacteria, Thermoleophilia, β-Alphaproteobacteria, Gammaproteobacteria, Spartobacteria, Saprospirae, and Actinobacteria at the class level; Rhizobiales, Gaiellales, Chthoniobacterales, Saprospirales, and Actinomycetales at the order level; Hyphomicrobiaceae, Gaiellaceae, Chthoniobacteraceae, Chitinophagaceae, and Bradyrhizobiaceae at the family level; Rhodoplanes, DA101, Bradyrhizobium, and Pseudomonas at the genus level. LEfSE analysis showed indicator bacteria in rhizosphere and non-rhizosphere soil, which were Yersinia, Thermogemmatisporaceae, Thermogemmatisporales, Spirosoma, NRP_I, Cellvibrio, Alteromonadaceae, MBGA, and TM1 in rhizosphere soil and Methylophilaceae, Methylophilales, Chromatiales, and ML635J_21 in non-rhizosphere soil.

