

Introduction
Antimony (Sb), an element with metalloid properties that is toxic and carcinogenic, is commonly acknowledged as a major environmental contaminant according to both the United States and the European Union [1-5]. Excessive levels of Sb in groundwater (>5.00 μg/L) are a global environmental concern across different regions worldwide, such as China [5, 6], Australia [7], Scotland [8], France [9], Canada [10, 11], Italy [12], and Egypt [13]. The primary natural routes for the infiltration of antimony (b) into groundwater were through oxidation and dissolution of Sb-bearing sulfides, such as stibnite (Sb2S3) and Jamesonite (Pb4FeSb6S14) [1, 11, 14-16]. Moreover, human activities such as mining and the burning of fossil fuels and waste materials have considerably enhanced the mobility and distribution potential of Sb in groundwater systems [16-19].
Dissolved organic matter (DOM) encompasses humic acids, fulvic acids, and proteins, which play a crucial role in the biogeochemical mobilization of Sb within groundwater [17, 20-24]. The presence of DOM could increase higher adsorption affinity for Fe hydroxide surfaces and facilitate the release of Sb [17, 25], while also forming complexes with Sb to improve its solubility [20, 21, 26, 27]. In addition, in the presence of sunlight, DOM have the potential to enhance the conversion of Sb(III) to Sb(V), thereby accelerating the movement of Sb in naturally occurring oxygenated environments [22, 23, 28]. The utilization of bio-reactive DOM had been found to enhance the autotrophic capabilities of microorganisms, thereby facilitating the oxidative dissolution of minerals containing Sb, such as stibnite [29, 30].
The molecular weight is widely recognized as a fundamental characteristic of DOM and plays a crucial role in influencing the interaction between DOM and metals [31-33]. In general, metals tend to exhibit a preference for DOM with varying molecular weights due to their distinct binding affinities [31, 33]. In natural aquatic environments, the mobilization of As is facilitated by its strong affinity for medium-molecular-weight DOM (MDOM) (1-10 kDa) and low-molecular-weight DOM (LDOM) (below 1 kDa) [32-35]. In addition to impacting the affinity for metal binding, amino acids containing LDOM exhibited bioactivity and were readily metabolized by microorganisms [36, 37].
Hence, comprehending the functional and molecular properties of DOM is crucial in investigating its involvement in the mobilization of As within natural aquatic environments. Despite the fact that As and Sb possess identical configurations of outer-orbital electrons (s2p3), it has been commonly assumed that their geochemical behaviors, which are influenced by DOM, tend to be similar [1, 17, 38]. Moreover, molecular weight fractions of DOM have been confirmed to affect the As mobilization in groundwater [17]. However, the impact of various molecular weight fractions of DOM on Sb pollution in groundwater remains poorly understood, thereby enhancing our comprehension of differences in Sb and As enrichment mechanisms within groundwater systems. Therefore, it is crucial to gain a comprehensive understanding of the source, characteristics, and geochemical reactivity of DOM with distinct molecular properties to elucidate the enrichment of Sb in groundwater.
The use of fluorescence spectroscopy has yielded significant knowledge regarding the nature, origin, and composition of DOM in groundwater [39-41]. Furthermore, the utilization of EEM-PARAFAC, a technique that combines excitation-emission matrix fluorescence with parallel factor analysis, has been extensively applied in identifying the origins and constituents of DOM owing to its quickness, cost-effectiveness, and accuracy [37, 42-45]. Recently, successful applications of molecular weight separation techniques have been observed in the assessment of metal distributions in DOM with different molecular weights in groundwater [32, 33, 46]. Changes in fluorescence offered valuable insights into identifying the unique fluorescence properties linked to different molecular weights of DOM [23, 33, 34].
Hence, the distribution and movement of Sb in shallow groundwater were investigated by analyzing the optical properties of DOM with varying molecular weights. This study aimed to (1) examine the spectroscopic characteristics and chemical properties of DOM with different molecular weights at various Sb concentrations and (2) assess the influence of DOM with different molecular weights on Sb mobilization in shallow groundwater. The findings from this study enhance our understanding of the mechanisms behind Sb enrichment in shallow groundwater.
Materials and Methods
Study Area
As the world’s largest antimony mine, the Xikuangshan mine is situated in central China, specifically 13 km north of Lengshuijiang City. It spans across a vast area of 26 km2 and is located within mountainous terrain that runs from northeast to southwest, with elevations ranging between 220 and 823.2 m. The climate is known for its high humidity, with an average annual precipitation of 1381.60 mm, evaporation reaching 903.30 mm, and temperatures averaging 16.7ºC from 1949 to 2012. The primary watercourses in the mining region that flow into the Zijiang River include the Xuanshan River, Qingfeng River, Feishuiyan Stream, Tanjia Stream, and Batangshan Stream. The Xikuangshan mine is internationally recognized as “The World’s Antimony Capital”, earning an impressive reserve of around 2.50 million tons of Sb [1, 17, 47, 48].
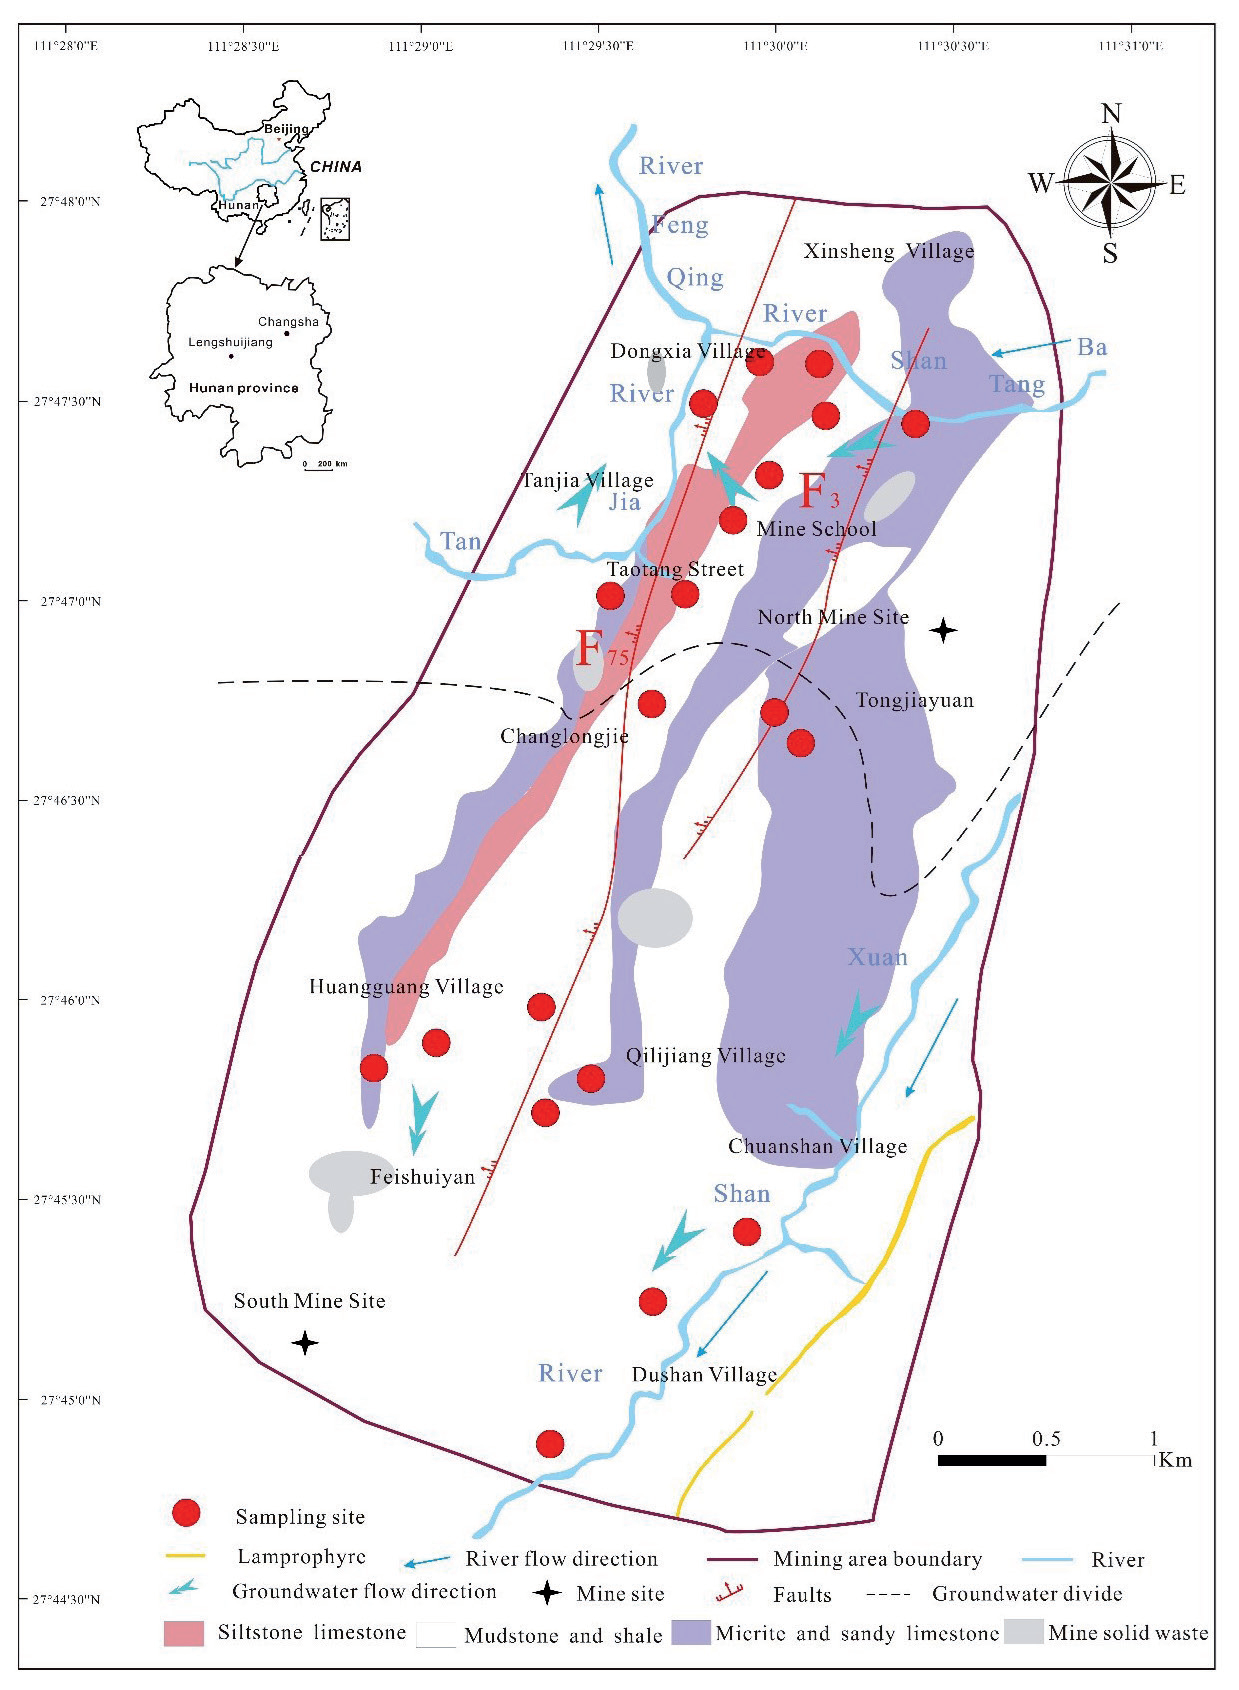
The Xikuangshan Sb mine area is situated in a hydrogeologically isolated region, enclosed by the NE30°-oriented fault NO.75 from the east and west. It encompasses a lamprophyre vein spanning approximately 10 km. As shown in Fig. 1, the primary aquifers in the mining region consist of the lower Shetianqiao karst aquifer (referred to as D3s2 water) and the upper Magunao karst aquifer (known as D3x4 water), which have been extensively studied by Wen et al. [5] (2016) and Hao et al. [1, 6]. The Sb ore bodies are located at the top of the silicified limestone layers of the D3s2 water, which have no hydraulic connection with D3x4 water. The D3x4 water, which consists of limestone and sandy limestone with an average thickness measuring 258 m and a hydraulic conductivity of 0.0092 m/d as reported by Wen et al.’s study conducted in 2016 and updated in 2022, plays a crucial role as a primary drinking water source for local residents. The main recharge source for the D3x4 water is infiltrated precipitation and agricultural irrigation, while groundwater flows from southeast to northwest in the North Mine and from northeast to southwest in the South Mine, respectively. D3x4 water discharge occurs through springs that crop out substantially and drainages associated with mining activities [4]. The primary hydrochemical facies in unpolluted D3x4 water is Ca-HCO3-SO4 type, and Sb concentration is less than 15 mg/L [4]. Some dwellings, industrial facilities, waste rock, and slag are situated over the D3x4 water [6, 49]. Moreover, mining regions extensively cultivate rice, corn, and vegetables as their main agricultural produce [17, 49].
Sample Collection
Based on the previous studies conducted on hydrogeology and geochemistry, a total of 20 springs were selected for sampling D3x4 water in February 2023 (Fig. 1a). Prior to collection, the brown plastic sampling bottles underwent sequential rinsing with distilled water and D3x4 water samples. All water samples were collected in the field and ultrafiltered sequentially through MilliPore filters (high-density polyethylene (HDPE)) with sequential pore sizes of 0.45-μm, 100- kDa, and 1-kDa by a cross-flow ultrafiltration system (CFUS, Sartorius Vivaflow®.200) [50].
Fig. 1.
Location of the study area and distribution of the D3x4 water sampling sites from the Xikuangshan mine.
Each of the filtered samples was separated into three categories: high-molecular-weight DOM (HDOM) D3x4 water (fraction<0.45 μm), middle-molecular-weight DOM (MDOM) D3x4 water (fraction<100 kDa), and low-molecular-weight DOM (LDOM) (fraction<1 kDa). A total of 60 D3x4 water samples were obtained during the process of ultrafiltration. The experiment involved utilizing a polymer-enhanced ultrafiltration system with a capacity of 300 mL by pressurizing and filtering with N2 gas. The ultrafiltration process was previously documented by Dundar et al. [51] and Li et al. [33]. To facilitate the analysis, the collected samples for the major cation and Sb analyses were treated with ultrapure HNO3 at a ratio of 1:1 (v/v) until reached a pH<2.0, after which they were promptly stored at a temperature of 4ºC in darkness. To prepare samples for stable organic carbon isotope analysis (δ13CDOC), they were acidified using 85% H3PO4 until the pH was less than 2. For stable inorganic carbon isotope analysis(δ13CDIC) was sterilized with HgCl2 and then collected in HDPE brown glass bottles with 100 mL.
Sample Analysis
The pH and total dissolved solids (TDS) were measured on-site at a sampling location using a portable pH meter (HANNA H18424, Italy) and a portable conductivity meter (HANNA H1833, Italy), respectively. The concentrations of bicarbonate ions (HCO3-) were determined by acid-base titration during field measurements with an analytical precision of 1.0 mg/L. Sb concentrations were determined using a hydride generation atomic fluorescence spectrometer (Qingdao) with a relative standard deviation of ±5% and an analytical precision of 0.10 µg/L [17, 28]. Total Fe (TFe) levels were determined using spectrophotometry (DR2800, HACH, USA) and the phenanthroline method with an analytical precision of 0.01 µg/L [17, 28, 52]. δ13CDOC and δ13CDIC in all samples were determined using isotope ratio mass spectrometry (Trace GC Ultra, Thermo Fisher Scientific, USA) coupled with an online high-precision gas headspace sampler, GasBench (Thermo Fisher Scientific), following the methods of Yu et al. [53] and Zhou et al. [54] with precisions<0.2‰.
The level of DOM was assessed utilizing a TOC- 5000 total organic carbon analyzer from Japan and represented as dissolved organic carbon (DOC), with an analytical accuracy of 0.01 mg/L. The UV-visible spectrophotometer (Hach DR-5000, USA) and the three-dimensional fluorescence spectrophotometer (F7000, Japan) were utilized to perform measurements of ultraviolet-visible and fluorescence in a 10-mm quartz cuvette. Both devices were equipped with a 150-W xenon lamp that does not emit ozone and operated at a consistent temperature of 20ºC. The emission wavelength (EM) was scanned from 220 to 550 nm while the excitation wavelength (EX) ranged from 200 to 400 nm, with sampling intervals of 5 nm during the excitation emission matrices (EEMs) analysis. The fluorescence measurements were conducted with an excitation wavelength step size of 5 nm and an emission wavelength step size of 2 nm. The scan rate was set at 2400 nm/min, the slit width was adjusted to 5 nm, and the amplification voltage used was 700 V.
The spectral overlap was determined by employing PARAFAC modeling with the assistance of fluorescence components from the DOMFluor database [55, 56]. All mean fluorescence intensities are calculated based on three repeated analyses, with subsequent subtraction of blank values and final normalization to Raman units (R.U.). The split half analysis and residual analysis were used to verify the reliability of the three-component model [33]. Residual intensities, were obtained by subtracting the PARAFAC-modeled EEM from the measured EEM maximum deviation of 10% compared to the measured EEM intensities across all samples.
To distinguish DOM sources, the fluorescence index (FI) was determined by dividing the measurement at an emission wavelength of 450 nm by that at 500 nm, after being excited at 370 nm, providing a metric for distinguishing DOM derived from terrestrial and microbial sources [32, 43, 57]. Furthermore, the biological index (BIX), which serves as a measure of indigenous biological activity in aquatics, was determined by dividing the emission intensities at wavelengths of 380 nm and 430 nm under a consistent excitation at 310 nm [58, 59]. In addition, the ratio of the emission scan at 435-480 nm to the emission scan at 300–345 nm with an excitation at 254 nm was utilized for evaluating the humification index (HIX), which serves as an indicator of DOM humification [60-62]. The calculation of the specific ultraviolet absorbance (SUVA254), which is linked to the aromatic nature of organic substances, involved normalizing the UV absorbance at 254 nm with respect to the DOC concentration [36, 59].
To enhance further characterization, the DOM was segregated into two categories. Initially, protein:humic ratios were computed by determining the proportion of protein-like DOM constituents in relation to the total sum of humic-like DOM components. Secondly, the microbial:terrestrial ratios were determined by calculating the proportion of DOM components derived from microorganisms compared to that of terrestrially derived DOM components.
Statistical Analysis
The statistical analysis software, Origin 2021, was employed to establish correlations among all findings. The PARAFAC analysis was performed using the DOM Fluor v.1.7 toolbox in MATLAB (Natick, MA, USA). Descriptive data can be found in Table 1, while Table 2 provides information on the spectroscopic characteristics of DOM components.
Table 1.
Geochemistry data for the D3x4 water of the Xikuangshan mine area.
Results
General Hydrochemistry Characterization
of D3x4 Waters with Different Molecular Weights
According to the geogenic values without pollution [5, 6], the D3x4 water samples were categorized into two groups: low-Sb groundwater (<15.00 µg/L) and high-Sb groundwater (>15.00 µg/L). pH values ranging from 7.14 to 9.74 with a mean of 8.03 were observed (Table 1), indicating a weakly alkaline environment in all D3x4 waters. The phenomenon indicated that H+ produced from stibnite oxidation had been immediately neutralized by carbonate minerals in D3x4 waters. The TDS concentrations in the high-Sb D3x4 water ranged from 121 to 1515 mg/L, with an average of 542 mg/L, surpassing those found in the low-Sb D3x4 water samples (ranging from 254 to 331 mg/L, with an average of 300 mg/L).
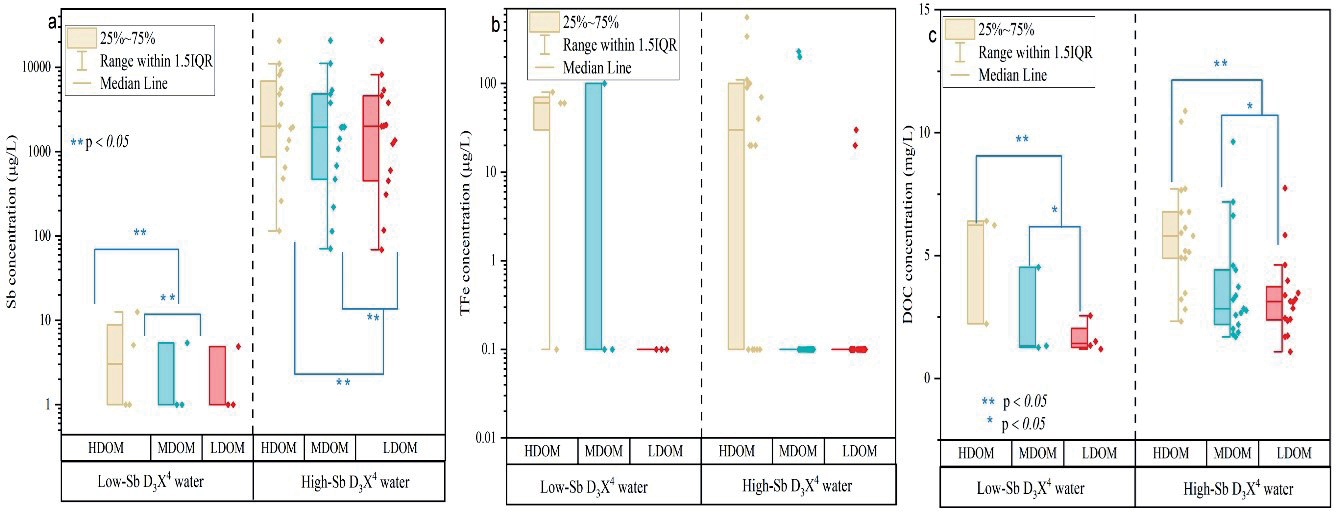
The concentration of Sb showed no significant differences among HDOM, MDOM, and LDOM in the low-Sb D3x4 water (Fig. 2a). There was a slight decrease during sequential ultrafiltration in the high-Sb D3x4 water, and a slight decrease was observed during sequential ultrafiltration in the high-Sb D3x4 water, suggesting that Sb predominantly existed as a truly dissolved form in the LDOM D3x4 water. These findings align with the research conducted by Zhang et al. [63] and Jia et al. [50] on Sb migration as well as the study by Li et al. [33] on As presence in shallow groundwater.
A decrease in DOM concentration was noted in LDOM and MDOM D3x4 waters compared to HDOM D3x4 water (Fig. 2c), suggesting that the HDOM D3x4 water exhibited the highest level of DOM content. The majority of TFe detected in the extracts was observed in the HDOM D3x4 water (Fig. 2b), which experienced a significant decrease in both MDOM and LDOM D3x4 waters. This suggested that TFe predominantly existed as large colloids within the HDOM D3x4 water [33, 35, 50, 63, 64]. The consistent trends between DOM and TFe indicate that TFe may have a higher affinity for binding with HDOM in the D3x4 water [35]. Earlier research had established that substances found in HDOM, such as humic-like and fulvic acids, exhibited a preference for forming DOM-Fe complexes with Fe hydroxides in groundwater [17, 35, 65, 66]. Therefore, it can be deduced that TFe predominantly exists as colloidal particles attached to HDOM in the D3x4 water [40]. However, the distribution of Sb in the D3x4 water with varying pore sizes exhibited distinct variations compared to the distributions of TFe and DOC as depicted in Fig. 2(a-c), indicating that HDOM was not a crucial factor for promoting Sb enrichment in the D3x4 water.
Fluorescence Characteristics of DOM with Different Molecular Weights
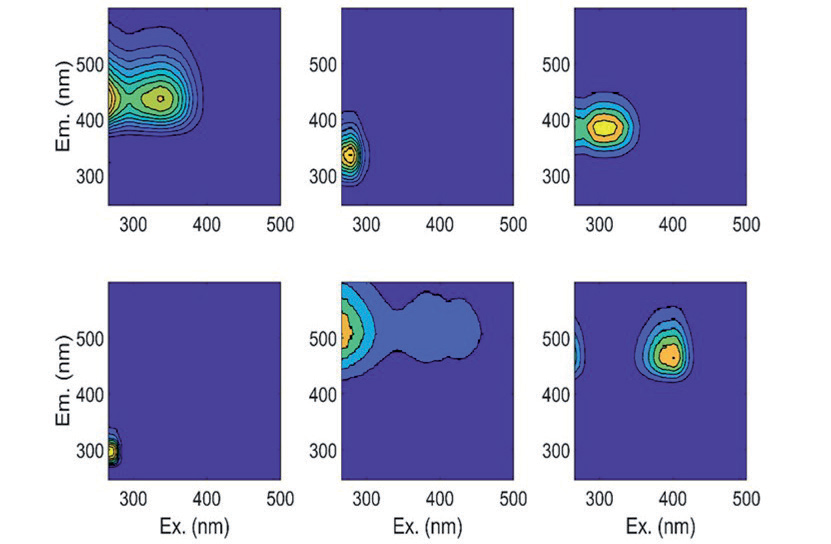
Fig. 3 showed the six main EEM peaks: Ex 266 (336)/Em 435 (Peak A, representing the C1 component) for the terrestrial humic-like component [37, 67, 68], Ex 278/Em 336 (Peak T, reflecting the C2 component) for the tryptophan-like substance [39, 69], Ex 306/Em 385 (Peak M, C3 component) for the microbial humic-like component [70, 71], Ex 266/Em 296 (Peak B, C4 component) for the carboxylic and phenolic groups component [32, 72], Ex 266/Em 507 (Peak C, C5 component) for the marine humic acid-like component [73, 74], and Ex 400/Em 464 (Peak D, C6 component) for the fulvic acid component [34, 64].
Table 2.
Descriptive statistics of the DOM components, SR, SUVA254, BIX, HIX, and FI in D3x4 water in the Xikuangshan mine area.
Fig. 2.
Box-whisker plots of Sb a), TFe b), and DOC c) for different size fractions of DOM in D3x4 water.
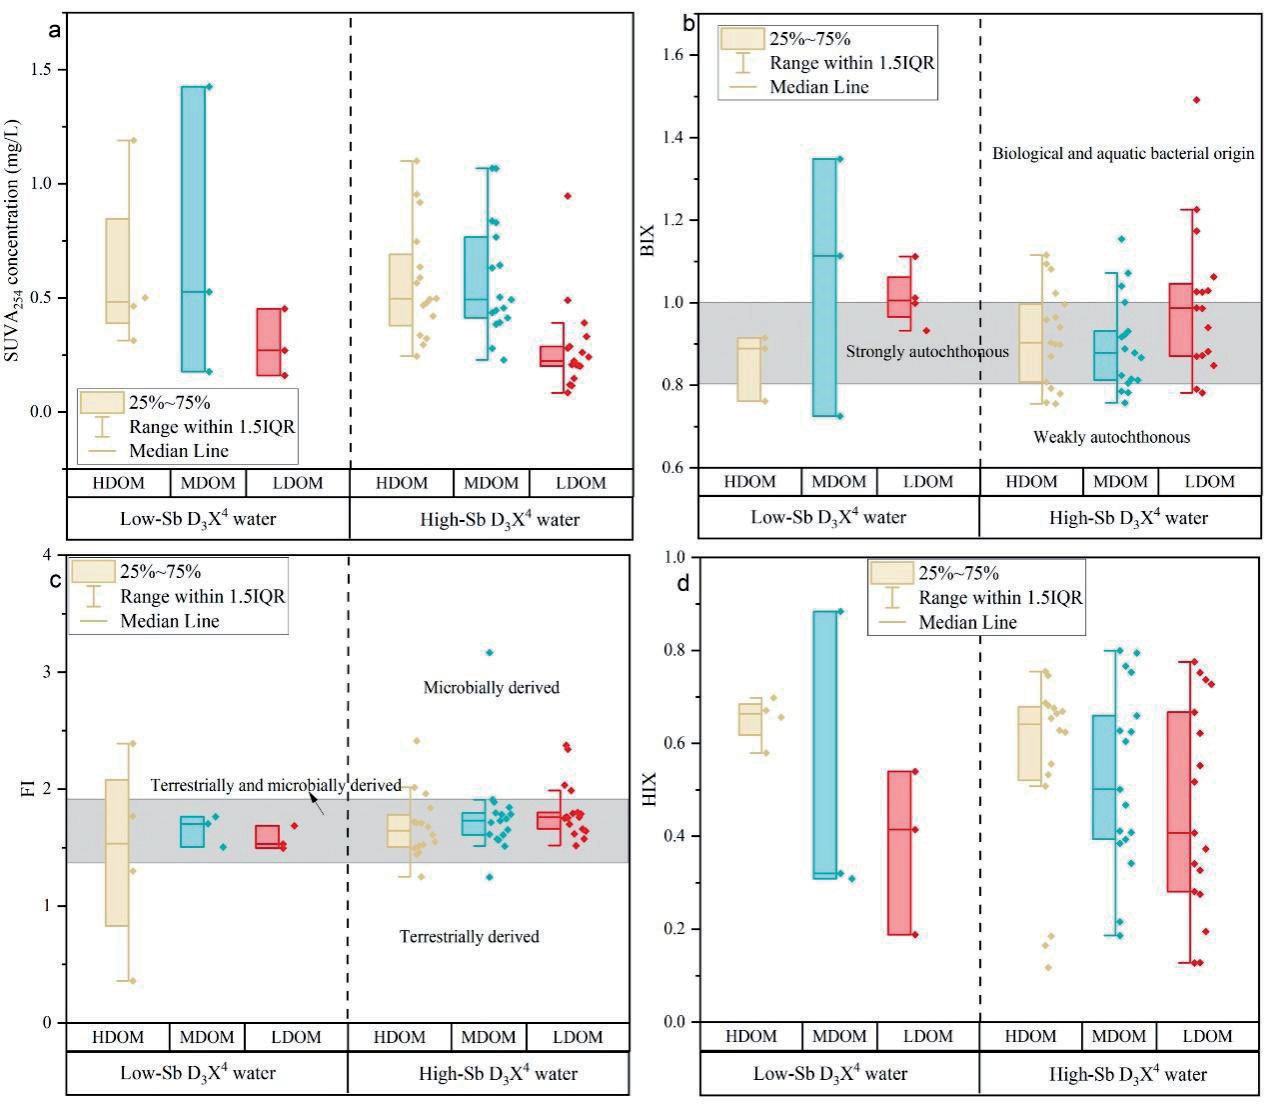
SUVA254, BIX, FI, and HIX of DOM with different molecular weights were shown in Fig. 4. During the process of sequential ultrafiltration, there was a slight increase observed in BIX, SUVA254, and HIX for low-Sb D3x4 waters (Fig. 4a–d), while a significant decrease was observed for high- Sb D3x4 waters. Significantly, the HDOM exhibited mean values of SUVA254 and HIX that were 2.65 and 1.27 times higher in the HDOM D3x4 water than those observed in the LDOM D3x4 water, respectively, suggesting a more pronounced presence of macromolecular aromatic substances in the HDOM D3x4 water. The rate of increase in BIX was found to be higher in the low-Sb D3x4 water compared to the high-Sb D3x4 water during the sequential ultrafiltration process (Fig. 4b), indicating the presence of biological and aquatic bacterial sources of DOM played a significant role in enriching Sb levels in the low-Sb D3x4 water [17, 27]. The FI values of both low- and high-Sb D3x4 water samples exhibited a wide range from 1.40 to 1.90, indicating the presence of terrestrial and microbial contributions (Fig. 4c). This suggests that the main sources of DOM in the D3x4 water are likely dominantly derived from terrestrial and microorganism origins [37, 43]. During the sequential ultrafiltration process, there was a slight transition in the FI values from terrestrially and microbially derived zones to microbially derived zones in high-Sb D3x4 water (Fig. 4c), suggesting a greater contribution from microbial sources in LDOM D3x4 water.
As indicated in Table 2 and Fig. 5a), the PARAFAC components of DOM were dominated by humic-like and fulvic acid components (the combined percentages of C1, C3, C5, and C6), followed by protein-like components (the sum percentages of C2 and C4) in HDOM and MDOM D3x4 waters, whereas the contents of protein-like components considerably increased and became predominant in the LDOM D3x4 water. The observation provided additional evidence that the protein-like constituents exhibited a progressive increase in dominance and promotion in the LDOM D3x4 water, whereas humic-like and fulvic acid components were predominantly present in HDOM D3x4 water throughout the sequential ultrafiltration process [17, 75]. Previous studies have established that the majority of humic-like and fulvic acid components are present in the colloidal fraction, which can be effectively captured through ultrafiltration utilizing membranes with a molecular weight cut-off of 1 kDa [35].
In Fig. 5b), the percentages of C2 and C4 significantly increased with the decrease in ultrafilter pore size, while the abundances of C1, C3, C5, and C6 declined during the sequential ultrafiltration process. For the given samples, there was a significant increase in the proportion of C4, accompanied by notable decreases in abundances of C1 and C3, when compared to the relative proportions of other components in the LDOM D3x4 water. This indicated that the LDOM D3x4 water contained a higher proportion of the tyrosine-like component, while the HDOM and MDOM D3x4 water favored the presence of humic-like components as large colloids [3, 40, 64]. The observed variations in the relative of the humic-like and fulvic acids, as well as protein-like components, were attributed to changes occurring during the sequential ultrafiltration process in Fig. 5a) and Table 2. As depicted in Figure 5c, the proportions of protein:humic and microbial:terrestrial progressively rose with the reduction in ultrafilter pore size, providing confirmation that the LDOM D3x4 water primarily contained a protein-like component derived from microorganisms.
In general, the HDOM D3x4 water exhibited higher levels of HIX, SUVA254, and percentages of C1 and C3, while lower levels of BIX, FI, and percentages of C2 and C4 were observed compared to the LDOM D3x4 water. This suggests that HDOM exhibited elevated levels of humification and aromaticity levels whereas LDOM was influenced by the microbial origin of DOM [33]. A similar outcome was observed in the high-As shallow groundwater with varying molecular weights in the Hetao Basin [33, 76], demonstrating that the chemical characteristics of DOM with distinct molecular weights may have similar effects on the fates of As and Sb.
Discussion
DOMs with Different Molecular Weights as a Complexing Agent for Sb
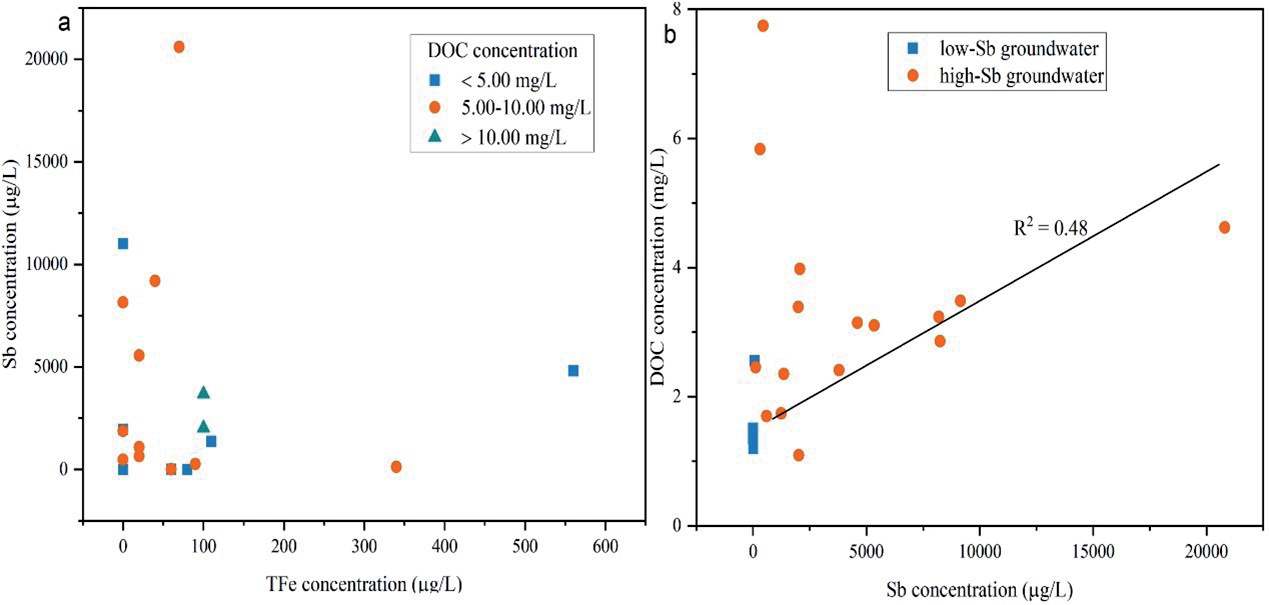
As depicted in Fig. 2a) and b), the majority of TFe was observed as Fe hydroxides in the HDOM D3x4 water, while Sb was predominantly present in the LDOM D3x4 water. Meanwhile, there were slight correlations between Sb, DOC, and TFe in the HDOM D3x4 water (Fig. 6a) and a significant positive correlation (R2 = 0.48) was found between Sb and DOC in the LDOM D3x4 water (Fig.6b), suggesting that the presence of enriched TFe hydroxides had minimal impact on the migration of Sb within the LDOM and MDOM D3x4 water. This contrasted with the findings of Li et al. [33] in their study on a high As groundwater from the Hetao basin, where they observed that higher binding capacity for As was demonstrated by larger Fe colloids (>10 kDa) during the sequential ultrafiltration process. The phenomenon implied that As exhibited a tendency to form stronger associations with Fe complexes compared to Sb, owing to DOM with different molecular properties.
Compared to low-Sb D3x4 water samples, TFe mean concentrations in high-Sb D3x4 water samples were found 3.14 times higher, indicating that Sb was likely associated with TFe hydroxides and complexes formed by DOM in high-Sb D3x4 water samples. Humic-like components could form DOM-Fe-Sb complexes by complexing with Fe hydroxides and Sb [17, 23, 63, 77]. This finding aligns with the observed higher values of HIX and SUVA254, as well as lower values of BIX and protein:humic ratio in the HDOM D3x4 water sample (Fig. 4a, b, d, and Fig. 5a). Complexes between Sb and humic-like substances of DOM are typically formed via the presence of positively charged amino groups in the DOM or metal cation bridges [20, 26, 40]. The interaction strength and durability of the binding between DOM and Sb were notably increased in groundwater through ligand substitution, the creation of negatively charged complexes, and the presence of bound hydrogen bridges [63, 78, 79].
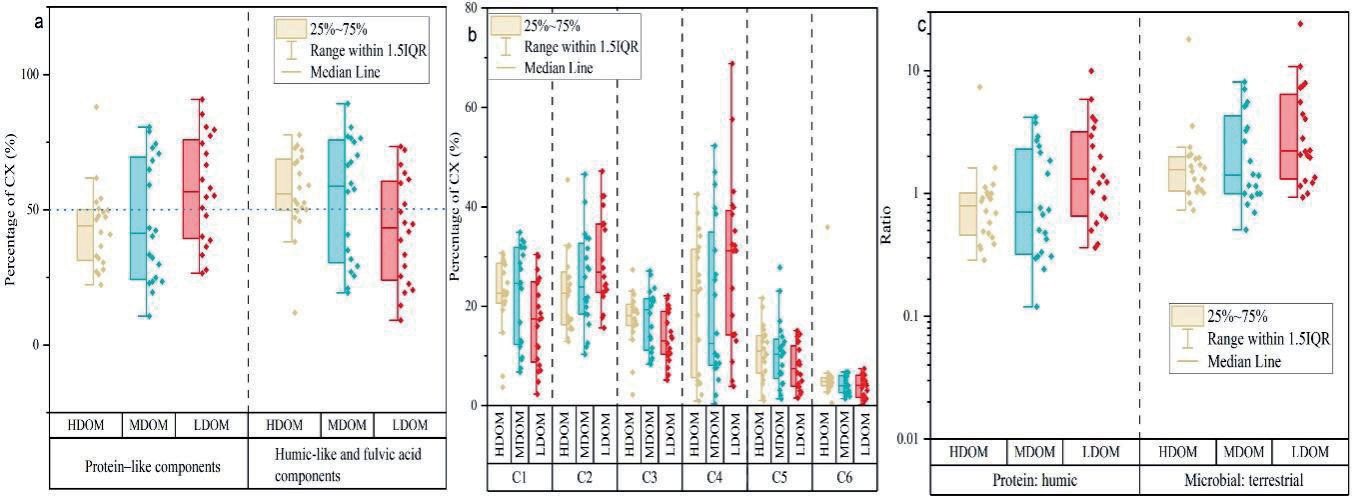
Fig. 6.
a) Sb versus TFe concentration in the HDOM D3x4 water and b) Sb versus DOC concentration in the LDOM D3x4 water.
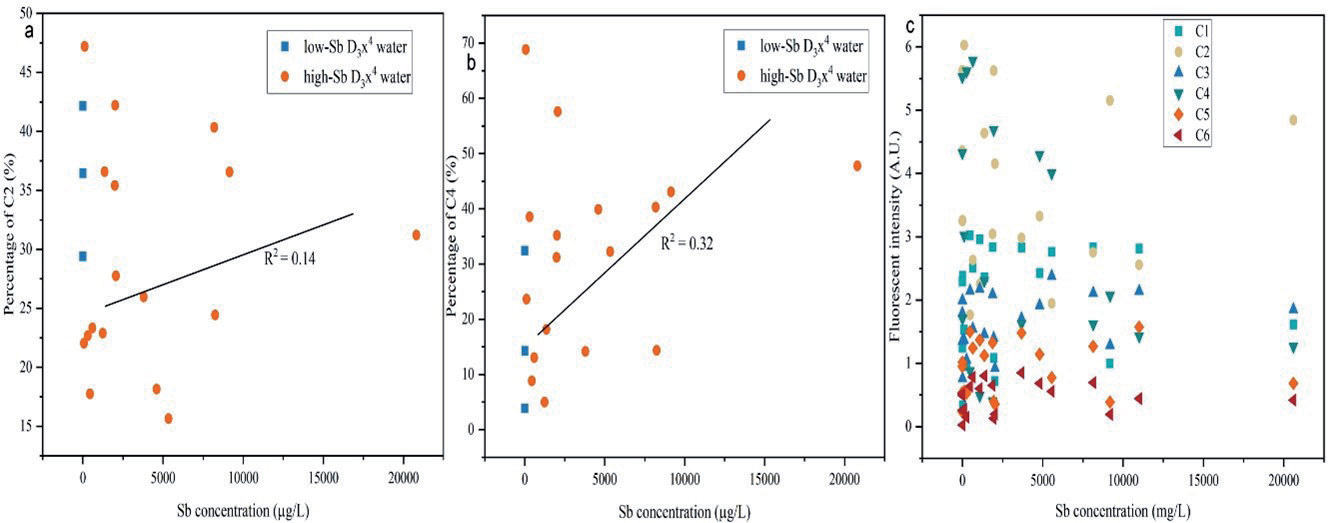
In addition, the Sb concentration in the LDOM D3x4 water showed weak (R2 = 0.14) and moderate (R2 = 0.32) positive correlations with the percentages of C2 and C4, respectively in Fig.7a and b. This suggested that protein-like component substances of DOM with lower HIX and SUVA254 and higher percentages of C2 and C4 may contribute to an increase in Sb levels in the LDOM D3x4 water. These protein-like substances are known for their strong affinity, such as copper and cadmium [20, 36, 80, 81]. Furthermore, the stable Sb(III) could be rapidly oxidized to an easily mobile Sb(V) in the presence of the quinone groups in neutral and alkaline waters, resulting in Sb concentration enrichment in the LDOM D3x4 water [23, 78, 82].
The changes in fluorescent intensity for the six PARAFAC-derived components during the increase in Sb concentration were illustrated in Fig. 7c), specifically focusing on the LDOM D3x4 water. The quenching curves exhibited a significant correlation with the origins of DOM sources. The initial decrease in fluorescent intensities of C4 and C2 was followed by a gradual decrease and stabilization as the concentration of Sb increased. Conversely, there was a slight increase in the fluorescent intensities of C3 and an increase in Sb concentration, which could be attributed to the combination of Sb with DOM [19, 83]. Weak quenching effects were observed for C1 and C6. These results suggested that the protein-like substances had more significant quenching effects than the humic-like materials in the LDOM D3x4 water.
In addition, the quenching levels of C4 were pronounced compared to those of C2, suggesting that the carboxylic and phenolic groups exhibited a stronger affinity for Sb in the LDOM D3x4 water [58, 81, 83]. Generally, the abundant presence of carboxylic and phenolic groups in DOM led to its high binding affinity towards heavy metals [58, 84], indicating the C4 component in the LDOM D3x4 water may be attributed to higher carboxylic and phenolic groups than other components. Moreover, the presence of carboxylic and phenolic groups on the C4 component may potentially hinder the adsorption onto TFe hydroxide surfaces, leading to the liberation of previously adsorbed Sb into the D3x4 water [17, 85].
Bioreactivity of LDOM and Microorganism Roles
Previous studies had proved the substances resembling proteins, characterized by a high BIX and low HIX and SUVA254 values, along with significant bioreactivity, were found to enhance the Sb mobility in groundwater systems by facilitating electron transfer and energy acquisition for microbial degradation and activities [30]. Generally, microbial degradation of organic matter causes a lower δ13CDIC and higher δ13CDOC in groundwater, reflecting an active microbial process [54, 86, 87].
As depicted in Fig. 8a), the <1 kDa fractions exhibited elevated δ13CDOC values and almost unchanged δ13CDIC values during the sequential ultrafiltration process, suggesting a more pronounced microbial influence on DOM within the LDOM D3x4 water. The observed fluctuations in δ13CDOC may be ascribed to the surface-driven microbial oxidation of organic substances occurring within the shallow groundwater. Extensive regions of rice, corn, and vegetables were allocated within the upper weathering zone of the D3x4 water. The input of DOM from precipitation may stimulate microbial respiration, resulting in an increase in δ13CDOC levels [88]. On the other hand, Sb with different valence states served as substrates for electron transfer and energy acquisition by autotrophic species in the oligotrophic groundwater environment [2, 30, 89]. The TFe levels in the LDOM D3x4 water varied from undetectable to 30.00 µg/L (with an average of 2.59 µg/L), creating favorable conditions for microbial degradation through its interaction with Fe oxides and DOM [33, 89]. Furthermore, oxidative stibnite, serving as the primary mineral containing antimony, could have potentially acted as a significant energy provider for autotrophic communities through the discharge of antimony and sulfur compounds into the D3x4 water environment [2, 30].
Fig. 7.
a) Percentage of C2, b) percentage of C2, and c) fluorescence intensity versus Sb concentration in the LDOM D3x4 water.
In Fig. 8b), a noticeable decline in the difference between δ13CDIC and δ13CDOC was observed in the LDOM D3x4 water as the Sb content increased (R2 = 0.72), suggesting Sb mobilization was related to the degree of microbial degradation of DOM [54, 90]. The lower difference between δ13CDIC and δ13CDOC suggests a higher level of microbial degradation of DOM, even though the isotopic variation in organic carbon is minimal and can be disregarded during microbial degradation processes [54, 91, 92]. The correlation between δ13CDIC and the difference between δ13CDIC and δ13CDOC was found to be significantly positive, indicating that the oxidative decomposition of organic carbon played an important role in the reduction in δ13CDIC. In the process of microbial degradation of DOM, microorganisms exhibited a preference for lighter carbon isotopes (12C), leading to decreased δ13CDIC levels and increased concentrations of HCO3- in groundwater [80, 93]. Compared to the low-Sb D3x4 water, the high-Sb D3x4 water exhibited lower and more negative δ13CDIC subtracted by δ13CDOC, indicating that the microbial degradation of DOM played a crucial role in the mobilization and enrichment of Sb in the LDOM D3x4 water [2, 17, 30].
Fig. 8.
a) Box-whisker plots of CX percentages for different size fractions of DOM, b) relationship between δ13CDIC - δ13CDOC and Sb concentration, and c) relationship between δ13CDIC - δ13CDOC and δ13CDIC in the LDOM D3x4 water.
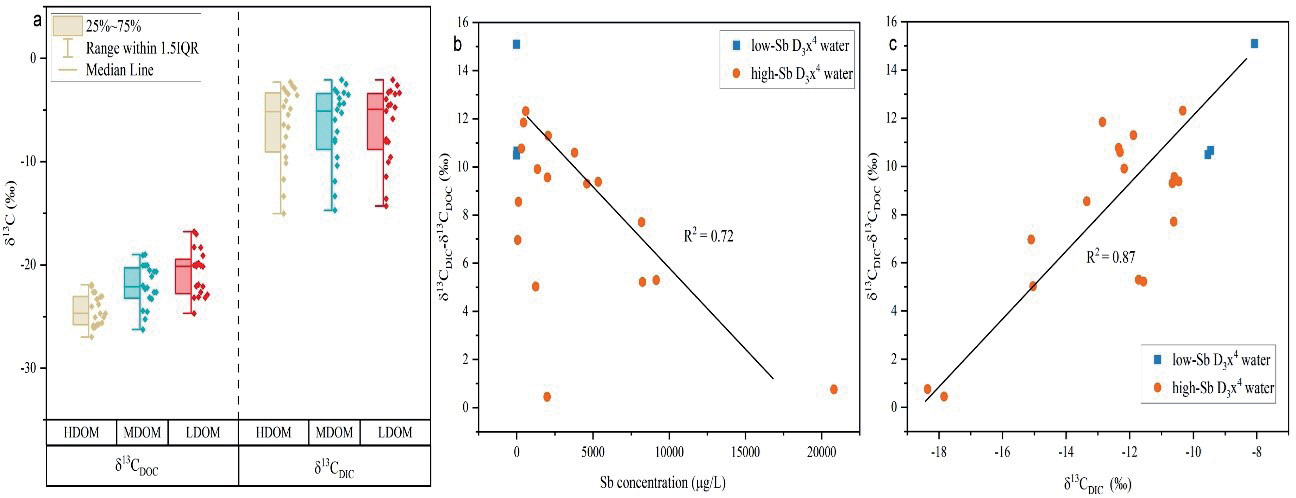
Fig. 9.
The sequential ultrafiltration process of DOM with different molecular weights for Sb migration in D3x4 water.
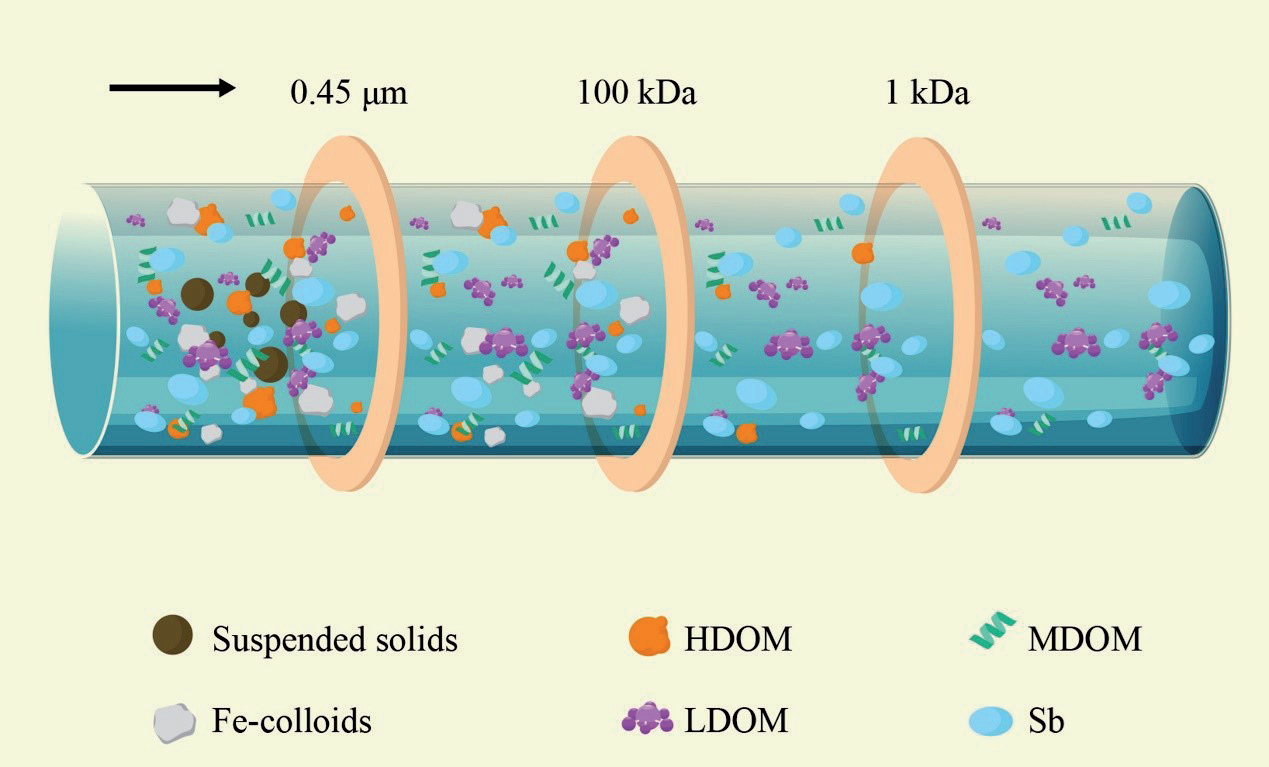
Therefore, our results suggested that Sb was primarily bound to protein-like substances with biological activity and is influenced by microbial degradation in the LDOM D3x4 water. As a result, the changes in Sb concentration were not found to be significant throughout the sequential ultrafiltration process (Fig.9). However, the impact of TFe was not ignored, which could play a role in facilitating the combination of Sb and DOM. This combination forms a Fe bridge, thereby promoting the accumulation of Sb in HDOM and MDOM D3x4 waters.
Conclusions
In this investigation, the majority of Sb was detected in the LDOM D3x4 water, while TFe colloids and DOC were mostly present in the HDOM and MDOM D3x4 water, respectively. The findings suggested that the presence of large Fe colloids or HDOM did not play a significant role in the enrichment of Sb in the D3x4 water. The LDOM D3x4 water, exhibiting elevated BIX and higher proportions of C2 and C4, and reduced HIX, percentages of C1 and C3 with a pronounced presence of protein-like substances, demonstrated compatibility for the formation of complexes with Sb. The quenching levels of C4 constituents generally surpassed those of C2, which showed that the carboxylic and phenolic groups exhibited an affinity for Sb in the LDOM D3x4 water.
During the sequential ultrafiltration process, higher δ13CDOC and lower δ13CDIC values were observed in the <1 kDa fractions. Additionally, in the high-Sb D3x4 water, there was a decrease in both δ13CDIC subtracted by δ13CDOC and δ13CDIC values. This suggests that microbial degradation of DOM played a significant role in influencing the mobility of Sb in the D3x4 water.
Despite molecular weight fractions of DOM may provide insights into its roles on Sb mobility, our findings are limited, and the molecular characteristics and mechanisms of DOM on Sb enrichment remain unclear. Overall, these discoveries will enhance comprehension of the biogeochemical actions of Sb and offer valuable perspectives for effectively managing shallow groundwater environments and ensuring the safety of drinking water within the study area.

