

Introduction
Alpine meadows in China are mainly distributed on the Qinghai-Tibetan Plateau and in the alpine belt of various high mountain systems, accounting for 22.1% of the national grassland area, which is one of China’s largest grassland types [1]. As an essential part of the global terrestrial ecosystem, alpine meadows are an important carbon source/sink, with soil organic carbon (SOC) reserves of about 33.5 Pg·C, accounting for 2.5% of the global SOC pool, but the area accounts for only 0.3% of the earth’s land area, which plays a pivotal role in the global carbon cycle [2]. Carbon stocks in alpine meadows of the Tibetan Plateau may have significant long-term impacts on the global carbon cycle [3]. However, the Tibetan Plateau is a sensitive and critical area for global climate change, which affects biogenic carbon by controlling the composition of plant communities, nutrient allocation strategies, microbial community composition, and biogeochemical processes. The Sanjiangyuan, known as the “Water Tower of China”, is the source of the Yellow River, Yangtze River, and Lancang River and plays an important role in water conservation and maintaining species diversity. The alpine meadows of the Tibetan Plateau are the main grazing lands for native herbivores, and grazing is common on the Tibetan Plateau to varying degrees [4]. In the late period of reform and opening up, scholars at home and abroad began to pay attention to the degradation of alpine grassland on the Tibetan Plateau caused by grazing [5]. The direct effect of grazing on alpine meadows is reflected in the reduction of plant height, cover, and biomass, resulting in a decrease in the amount of litter material entering the soil. There are differences in the amount of litter matter returning to the surface and entering the soil in alpine meadows under different grazing treatments [6]. These differences may disrupt the original nutrient balance of alpine meadow ecosystems.
Soil microbial biomass carbon (MBC) is the most active and variable part of soil organic matter, accounting for only 0.3%~9.9% of total soil carbon, is the driving force of SOC and nutrient transformation and cycling, and is directly involved in the decomposition and transformation of organic carbon, which is the soil nutrient reserve and an important source of nutrients for plant growth [7]. Soil microbial biomass carbon pools (MBCP) are the sum of carbon elements in the bodies of all microorganisms (including bacteria, fungi, actinomycetes, protozoa, algae, etc.) in the soil. As a link between aboveground vegetation and belowground soil, litter plays an important role in nutrient metabolism and cycling in the plant-soil system through different rates of nutrient return and decomposition [8].
As a major nutrient supplier to alpine meadow ecosystems, litter is critical for storing microbial biomass carbon pools. Litter input and removal treatments have been widely used as an effective experimental method for evaluating the effects of litter on soil microbial biomass and community structure in terrestrial ecosystems [9, 10]. The estimation of MBCP mostly relies on models; nevertheless, the limitations of conventional models in highland environments lead to their inability to accurately estimate and predict changes in carbon pools. For example, the simplifying assumptions of the Rothamsted carbon model are not suitable for influencing the estimation and prediction results of the model due to the extreme climate, low oxygen, and freeze-thaw cycles in the Sanjiangyuan area [11]. Increased litter inputs have been found to increase MBC content [12, 13]. It was also found that litter inputs had no significant effect on MBC content [14]. Nevertheless, most of the existing studies have focused on qualitative studies on the effects of litter inputs on plant community structure and function in temperate grasslands and typical grasslands [15, 16], and there is a lack of targeted studies on the effects of litter inputs on MBCP in alpine meadows. Few studies have been reported on how litter inputs affect MBCP in alpine meadows.
Therefore, alpine meadows were selected as the research object in this study. By simulating the effects of different levels of litter inputs on MBCP in ungrazed, lightly grazed and moderately grazed alpine meadows, we set up experiments with different levels of litter inputs (T0 (CK), 20% of standard (T1), 50% of standard (T2) and 100% of standard (T3)) to analyze the dynamic changes of soil physicochemical properties, enzyme activities, microbial biomass, and MBCP under different levels of litter inputs, focusing on the following scientific issues: (1) the dynamic changes of soil physicochemical properties, enzyme activities, microbial biomass, and MBCP under different litter treatments in ungrazed, lightly-grazed and moderately-grazed alpine meadows, and (2) to reveal the key factors affecting MBCP in ungrazed, lightly grazed and moderately grazed alpine meadows under liter input. This study can provide microbial mechanism parameters for the alpine meadow carbon cycle model, optimize the regional carbon balance assessment tool, and provide a theoretical basis for sustainable management of alpine meadows.
Materials and Methods
Overview of the Study Area
This study was carried out in accordance with the construction of the Suedo substation of the Qinghai Sanjiangyuan Grassland Ecosystem National Field Scientific Observation and Research Station. Referring to the classification standard of Technical Regulations for Yak Grazing Utilization in Alpine Meadows (DB63/ T607-2006) issued by the Qinghai Provincial Bureau of Quality and Technical Supervision [17], which was drafted by the Northwest Plateau Institute of Biology of the Chinese Academy of Sciences and the Qinghai Academy of Animal Husbandry and Veterinary Science), which was drafted by the Northwest Plateau Institute of Biology of the Chinese Academy of Sciences and the Qinghai Provincial Academy of Animal Husbandry and Veterinary Science, classifies alpine meadows as ungrazed, lightly grazed and moderately grazed alpine meadows based on criteria such as dominant species of plant communities and graminoid cover (Table 1).
Experimental Design
In order to study the effects of different levels of litter inputs to MBCP in alpine meadows under ungrazed, lightly grazed, and moderately grazed alpine meadows, the present study selected sample plots in the study area to conduct the experiment. The area of each plot was 4 m2 (2×2 m). In grassland ecosystems, more than 90% of the net production of plants is returned in the form of litter [18]. In view of this, this study is based on the results of the previous research on alpine meadows in the Sanjiangyuan District [19], as well as combined with the current situation of the experimental area; at the same time, reference is made to the published literature [20, 21]. The glucose addition in this experiment was based on 2% APC (Aboveground Community Carbon Content of Vegetation). Four treatments were set up in this study: 20% of the standard amount (T1), 50% of the standard amount (T2), 100% of the standard amount (T3), and T0 (CK). The plot area was 2×2 = 4 m², the plot interval was 1 m, and there were 4 replications, totaling 4×4 = 16 plots. Three types of grassland, namely, fenced (F), lightly grazed (L), and moderately grazed (M), totaled 48 plots (Table 2).
Table 1.
Classification of alpine grassland degradation and sample sites.
Sample Collection
Sampling was carried out at the end of September 2024 during the growing season of the plants in the above test area.
Plant Biomass and Soil Collection
We set up 1×1 m sample plots for plant and soil sample collection in the experimental area. Aboveground plants were mowed flush with the ground, packed into envelopes, and placed in a cool place; belowground biomass was collected from the 0~30 cm soil layer using a soil auger with an inner diameter of 5 cm, and the samples were packed into envelopes and bags, brought back to the laboratory to remove gravel and sand, and then the roots were separated using a standard soil sieve of 0.28 mm aperture and rinsed and air-dried. Samples were taken 5 times and mixed into 1 sample.
The soil samples were collected by the soil auger method [22] from 0~30 cm soil layer in the sample plots where the aboveground plant characteristics had been sampled. The soil samples from each sample plot were mixed 5 times with an auger of 5 cm internal diameter to form a single sample. 5 replicates were made. The soil samples were transported back to the laboratory, mixed and sieved, and placed in a cool, ventilated place to air dry before being used to determine soil NH₄⁺ and NO₃⁻.
Measurement and Calculation of Indicators
Measurement of MBC and MBN Content
Referring to Vance et al. (1987) [23], Determination using the chloroform fumigation leaching method. Each soil was divided into two portions; one was fumigated in a vacuum desiccator for 24 h, and the other was not fumigated. Both fumigated and unfumigated soils were leached with 0.5 mol/L K2SO4 (water-soil ratio: 4:1, 40 mL of 0.5 mol/L K2SO4 solution, 10 g of fresh soil), and the leachate was filtered and then sucked up into 10 mL to 50 mL bottles and then analyzed by a TOC analyzer (Warip TOC SELECT) to determine the MBC content. The MBC content was finally calculated from the difference between the fumigated and unfumigated values, with a conversion factor of 0.45 for MBC.
MBCP Calculation
MBCP is calculated by the following formula [24]:
MBCP (g/m2) = MBC (mg/kg) × BD (g/cm3)
× H (cm) × 10
In the formula, H denotes the thickness of the soil layer.
Determination of Soil Physical and Chemical Properties
The soil’s three parameters, soil moisture (SM), soil electrical conductivity (EC), and soil temperature (ST), were measured and recorded using a three-parameter meter (Spectrum, U.S. TDR 350) at 3.8 cm and 7.6 cm in each experimental plot.
Soil pH: pH meter method.
Measurement of Enzyme Activity
Litter input not only affects the growth of alpine meadow plants but also influences the soil environment and directly affects the dynamics of soil microbial communities. Plant-microbe interactions in ecosystems can be predicted by changes in soil enzyme activities [25]. The major enzymes include soil hydrolase (S-FDA), glucose oxidase (GOD), soil dehydrogenase (S-DHA), β-1,4-glucosidase (S-β-GC), cellobiose hydrolase (CBH), and β-1,4-xylosidase (S-β-XYS). Measurements are referenced in the literature [26-31].
Soil Bulk Weight
Measured by the ring knife method [32]. The formula is as follows: Soil Bulk Weight (g/cm3) = Quality of Dried Soil (g)/
Data Processing
Microsoft Excel 2016 was used to organize the raw data. All data were tested for normality and chi-square, and one-way ANOVA analysis and Tukey’s multiple comparisons were used to determine the differences between different levels of litter inputs on soil physicochemical properties, soil enzyme activities, and microbial biomass of alpine meadows, with significant differences assessed at the level of P<0.05. Relationships between indicators of soil physicochemical properties, soil enzyme activities, and microbial biomass were analyzed using correlation analysis. Structural equation modeling with composite variables was constructed using the “nlme” and “piecewise SEM” packages in R 4.4.3, which nested mixed-effects models to investigate the effects of soil physicochemical properties, soil enzyme activities, and soil microbial biomass on MBCP in alpine meadows. The model was nested with a mixed-effects model to investigate the direct and indirect effects of soil physical and chemical properties, soil enzyme activities, and soil microbial biomass on MBCP. All statistical analyses were done in R 4.4.3, and statistical graphics were done in Origin Pro 2021.
Results
Effects of Litter Input on Soil Physicochemical Properties in Alpine Meadows
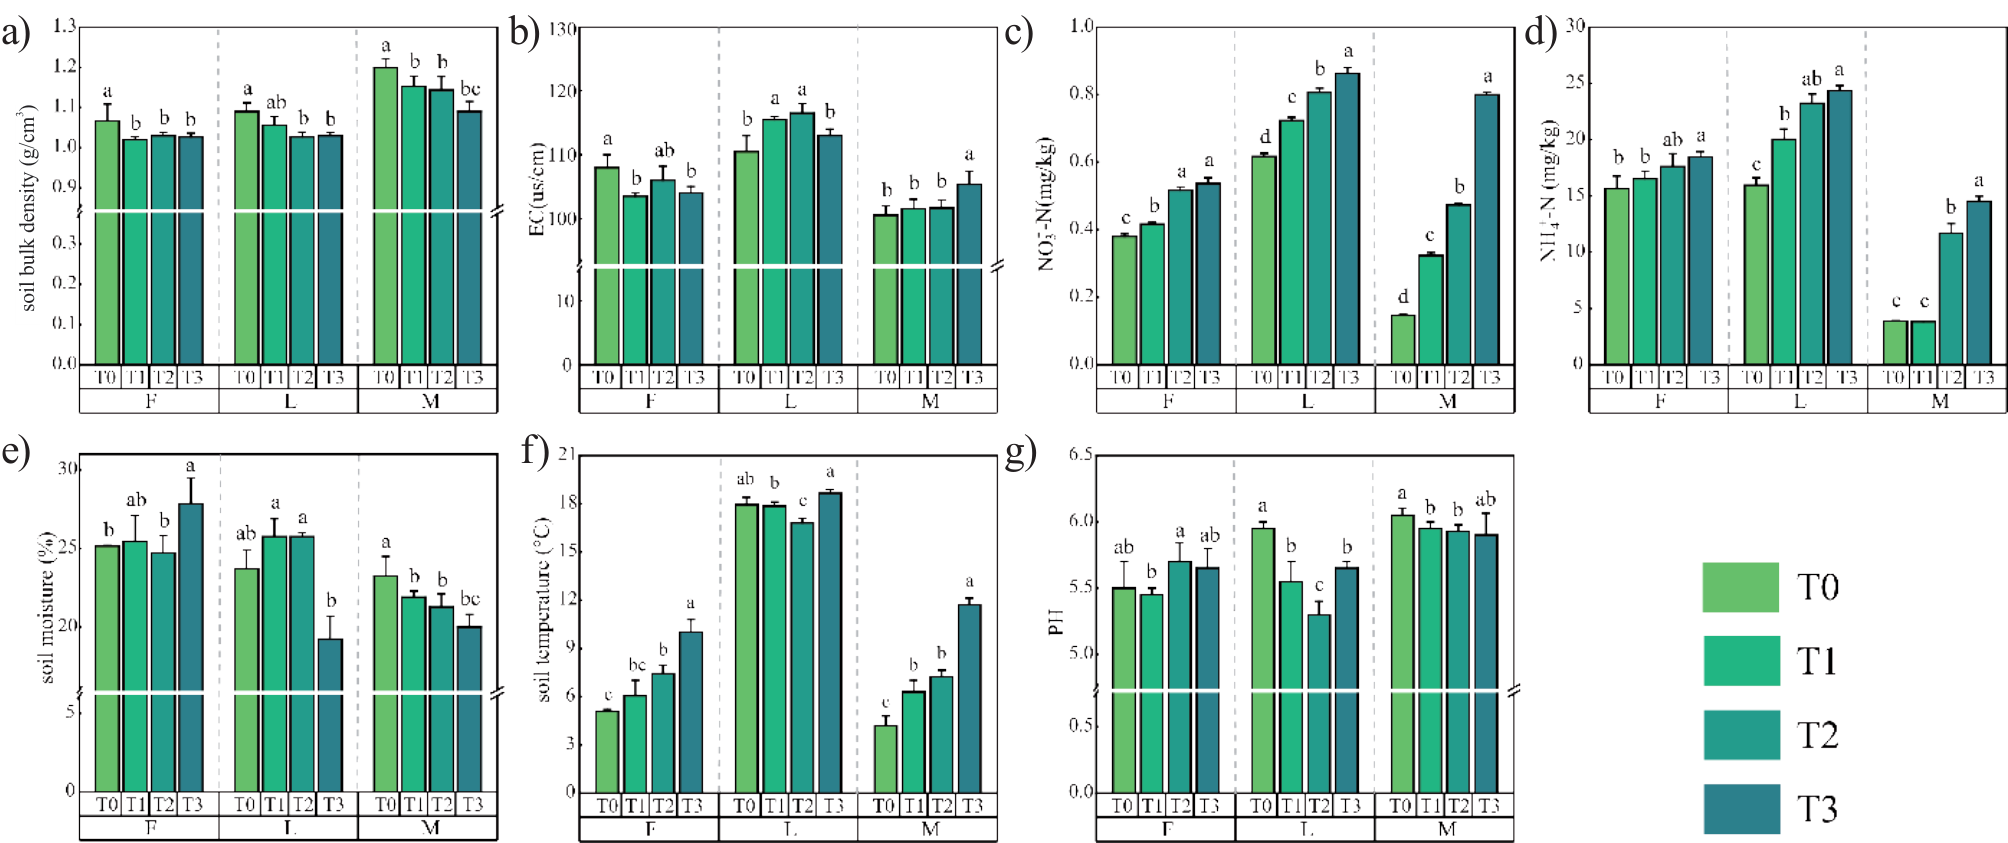
The physical and chemical properties of ungrazed, lightly grazed, and moderately grazed alpine meadow soils showed significant dynamic changes under different levels of litter input (P<0.05). The soil temperature of ungrazed and moderately grazed alpine meadows showed a significant positive effect, which peaked at T3 (Fig. 1a)). NH₄⁺-N and NO₃⁻-N showed an overall trend of gradual increase under litter inputs, both of which peaked at T3. Lightly grazed was higher than ungrazed and moderately grazed, with the maxima being 24.89 mg/kg and 0.86 mg/kg, respectively (Fig. 1f) and g)). Soil bulk density showed a gradual decrease under different levels of litter input (Fig. 1e)). SM, EC, and pH did not show a uniform pattern of change under litter input, and the differences were significant (P<0.05) (Fig. 1(b-d)).
Effects of Litter Inputs on Soil Enzyme Activities in Alpine Meadows
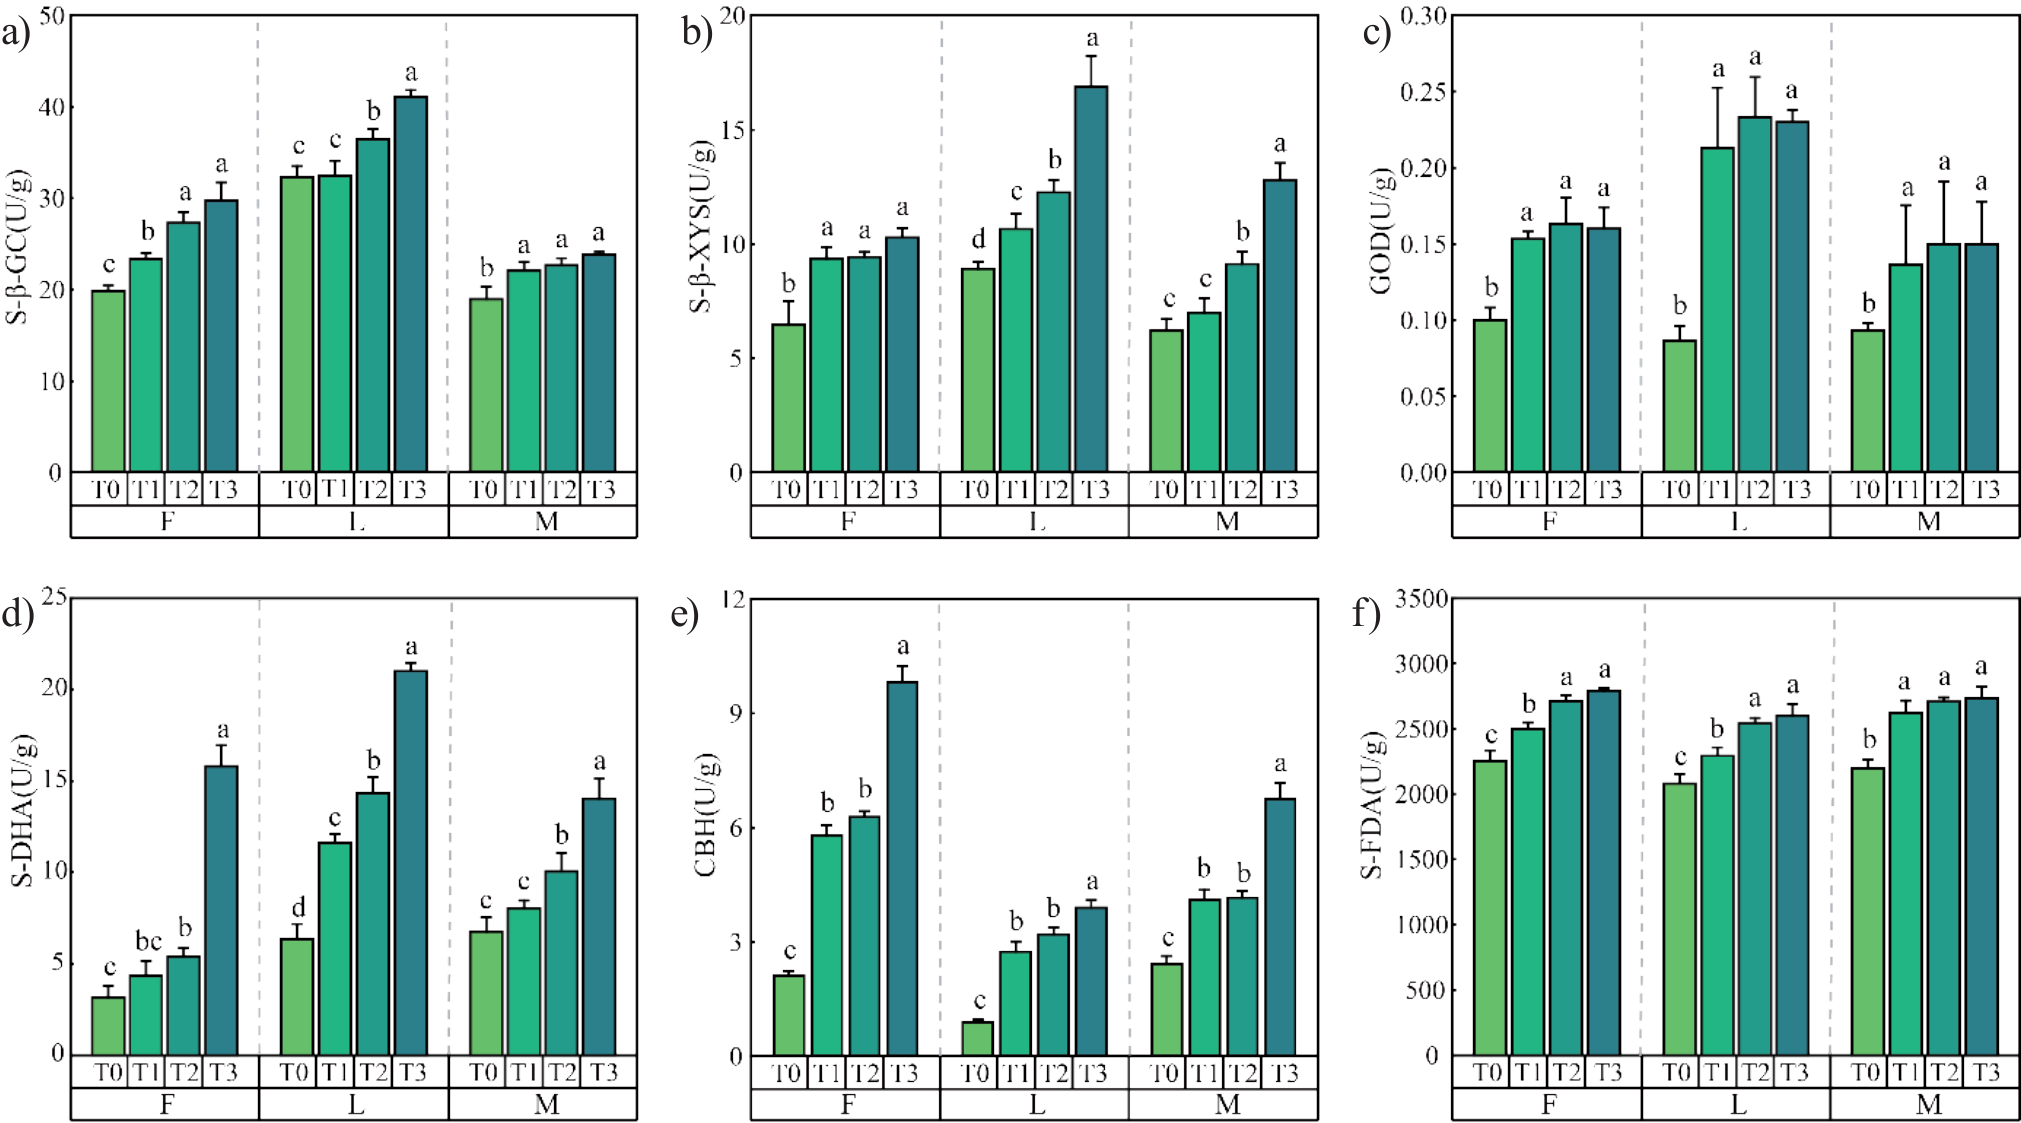
As shown in Fig. 2, the soil enzyme activities of ungrazed, lightly grazed, and moderately grazed alpine meadows showed similar change patterns under different litter input levels, with significant differences (P<0.05). With the increase of litter input, S-β-XYS, S-β-GC, S-FDA, S-DHA, and CBH showed a gradual increase, and all of them had a maximum value at T3 (Fig. 2a), b), d), e), and f)). S-β-XYS, S-β-GC, GOD, and S-DHA values under light grazing were higher than those under ungrazed and moderate grazing. The peak values of S-β-XYS, S-β-GC, and S-DHA were at T3, which were 16.87 U/g, 41.09 U/g, and 21.01 U/g, respectively (Fig. 2a), b), and e)).
Effects of Litter Input on MBC and MBN Content and MBC/MBN in Alpine Meadows
The MBC and MBN contents of MBC/MBN of ungrazed, lightly grazed, and moderately grazed alpine meadow soils showed significant dynamic changes under different levels of litter input (P<0.05). With different levels of litter input, the MBC and MBN contents gradually increased to an “upward” trend, and all peaked at T3. Lightly grazed MBC content was greater than that of ungrazed and moderately grazed, with a maximum value of 605.77 mg/kg (Fig. 3a)). Ungrazed MBN content was greater than light and moderate grazing, with a maximum value of 55.11 mg/kg (Fig. 3b)).
However, there was no regular dynamic change in the values of MBC/MBN of ungrazed, lightly grazed, and moderately grazed alpine meadow soils, and the values of MBC/MBN of ungrazed and moderately grazed soils showed a gradually decreasing dynamic trend with the increase of litter inputs. The values of MBC/MBN of ungrazed soils were larger than those of moderately grazed soils, with a maximum value of 20.8 (Fig. 3c)).
Effects of Litter Input on MBCP in Alpine Meadows
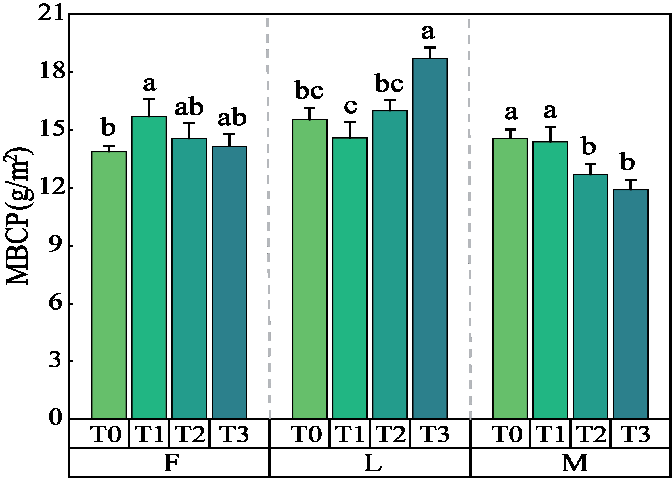
As shown in Fig. 4, MBCP of ungrazed, lightly grazed, and moderately grazed alpine meadow soils showed significant dynamic changes under different levels of litter input (P<0.05). MBCP was higher in lightly grazed than in ungrazed and moderately grazed and peaked at 18.72 g/m2 at T3.
Correlations between Physical and Chemical Properties, Enzyme Activities, and Microbial Biomass in Alpine Meadows
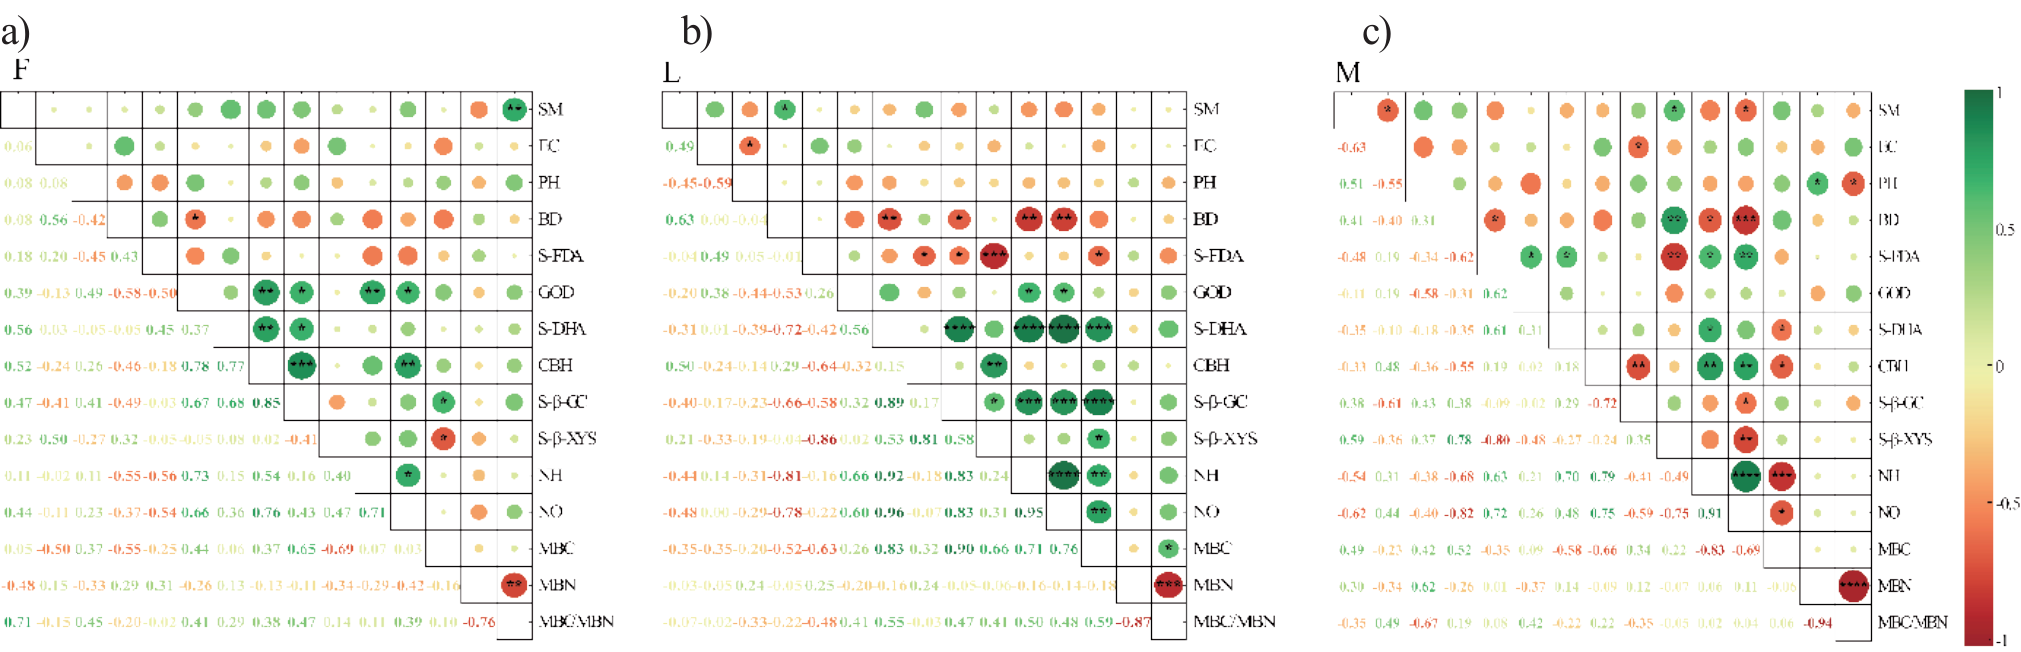
The above studies investigated the dynamic changes of soil physicochemical properties, soil enzyme activities, and microbial biomass in ungrazed, lightly grazed, and moderately grazed alpine meadows. To further investigate the correlation among the physicochemical properties, enzyme activities, and microbial biomass of alpine meadow soils, correlation analyses revealed that there was a significant positive correlation between SM and MBC/MBN in ungrazed alpine meadow soils and that GOD showed a significant positive correlation with CBH, S-β-GC, NH₄⁺-N, NO₃⁻-N, and S-DHA showed a significant positive correlation with CBH and S-β-GC. CBH showed a significant positive correlation with S-β-GC and NO₃⁻-N, and MBC showed a significant negative correlation with S-β-XYS (P<0.05) (Fig. 5a)).
Fig. 3.
Effect of litter input on MBC, MBN, and MBC/MBN in alpine meadows. Note: Lowercase letters in the figure represent significant differences between treatments (P<0.05).
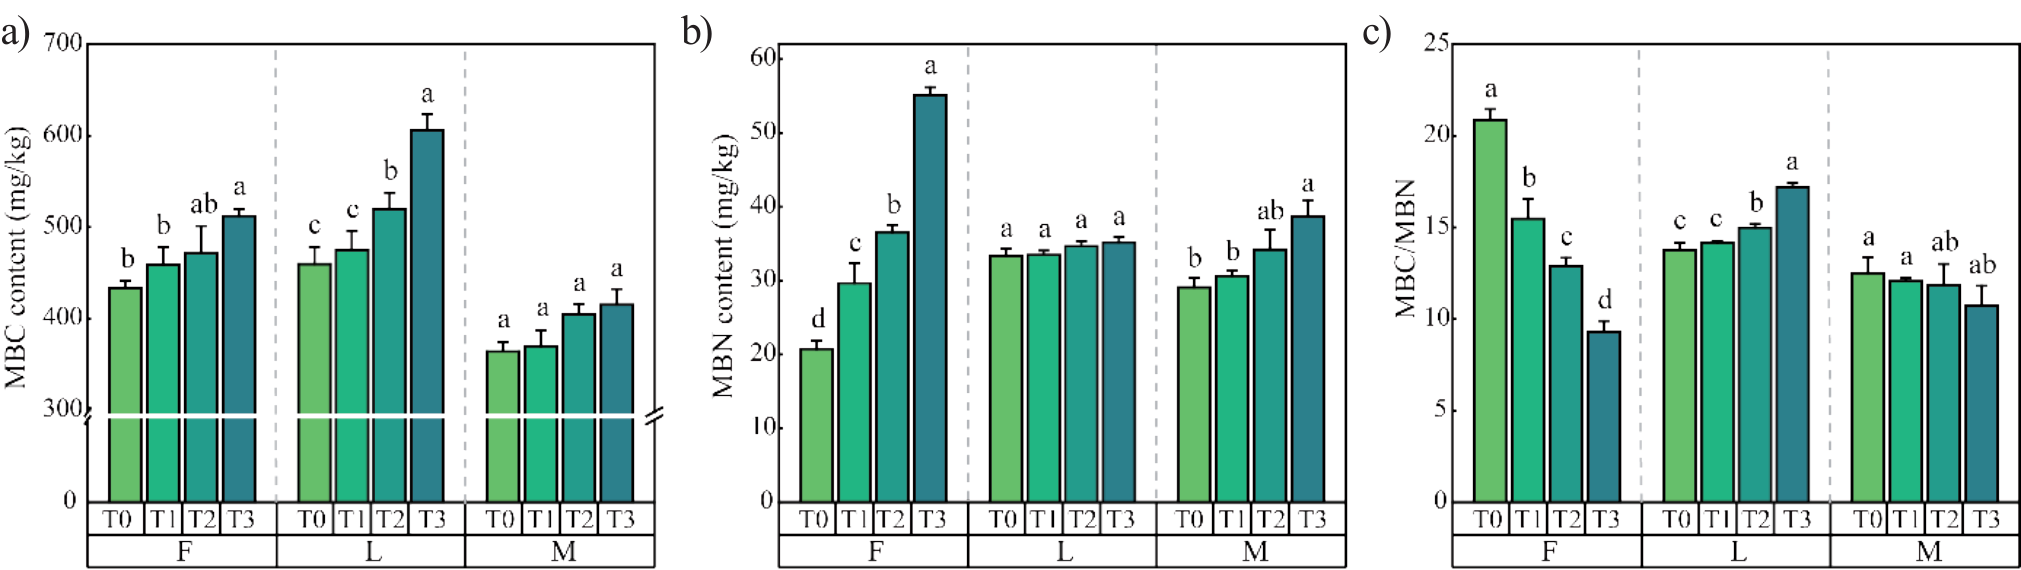
Fig. 4.
Effect of different levels of litter inputs on MBCP in alpine meadows. Note: Lowercase letters in the figure represent significant differences between treatments (P<0.05).
Lightly grazed alpine meadow BD showed a significant negative correlation with S-DHA, S-β-GC, NH₄⁺-N, NO₃⁻-N, and S-FDA showed a significant negative correlation with CBH, S-β-GC, S-β-XYS, and MBC. S-DHA showed a significant negative correlation with S-β-GC, NH₄⁺-N, NO₃‾, and MBC; S-β-GC was significantly positively correlated with S-β-XYS, NH₄⁺, NO₃⁻, and MBC (P<0.05) (Fig. 5b)). Moderately grazed alpine meadow soil, S-FDA, was significantly and positively correlated with GOD, S-DHA, NH₄⁺-N, NO₃⁻-N, and CBH was significantly and positively correlated with NH₄⁺-N and NO₃⁻-N. BD was significantly correlated with S-FDA, NH₄⁺-N, and NO₃⁻-N; there was a significant negative correlation (P<0.05); CBH had a significant negative correlation with S-β-GC and MBC (P<0.05) (Fig. 5c)).
Structural Equation Modeling of MBCP in Alpine Meadow Soils under Litter Input
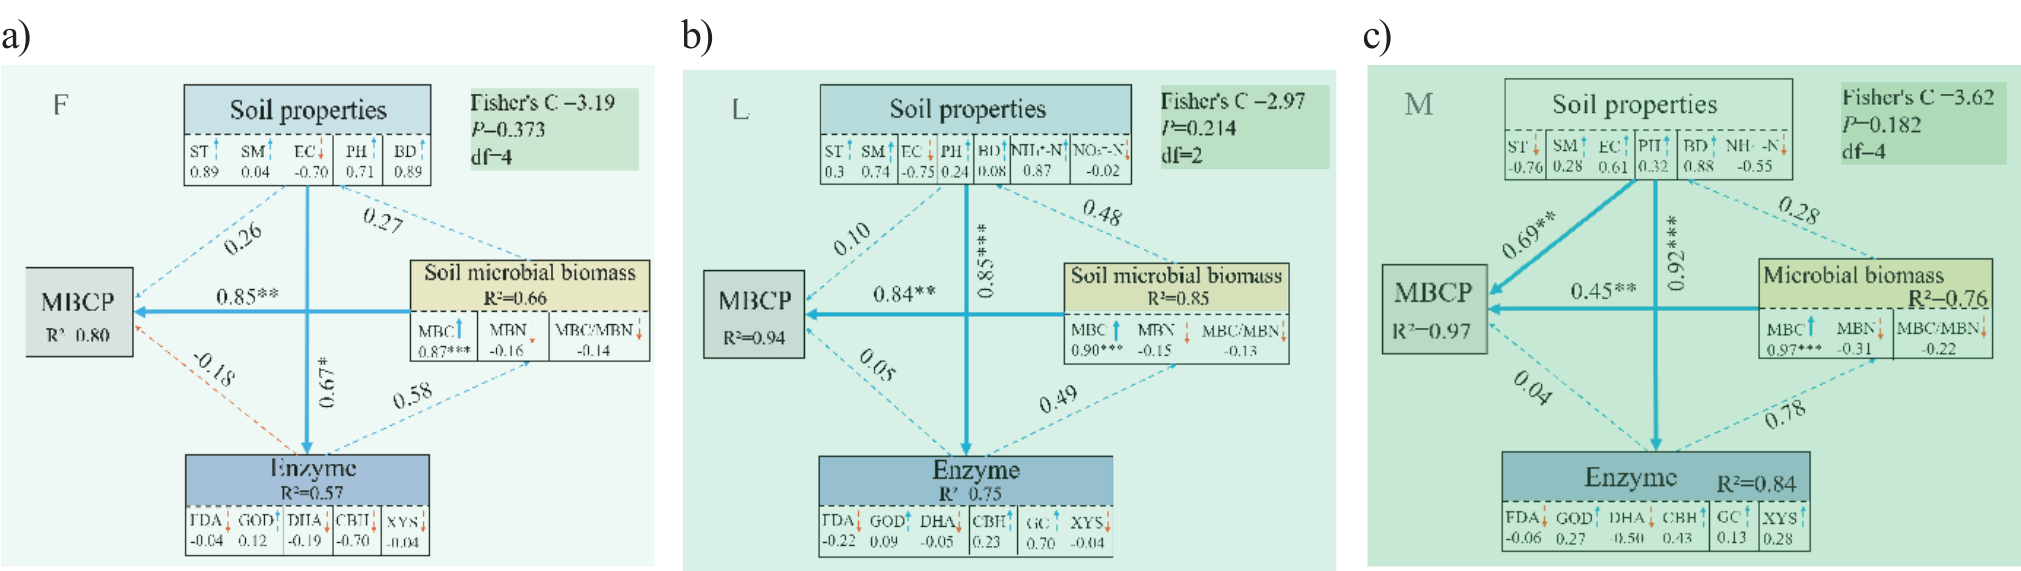
This study used structural equation modeling combined with mixed-effects modeling to investigate the effects of ungrazed, lightly grazed, and moderately grazed alpine meadow soil physicochemical properties, soil enzyme activities, and soil microbial biomass on MBCP, respectively. As can be seen from Fig. 6, the structural equation models fitted well (F: Fisher ʹC = 3.19, P = 0.372, df = 4; L: Fisher ʹC = 2.97, P = 0.214, df = 2; M: Fisher ʹC = 3.62, P = 0.182, and df = 4), indicating that the models effectively explained the MBCP and soil physicochemical properties, soil enzyme activities, and soil microbial biomass.
Fig. 5.
Correlation between physicochemical properties, enzyme activity, and microbial biomass of alpine meadows.
Soil microbial biomass in the ungrazed, lightly grazed, and moderately grazed alpine meadows showed a significant positive effect on MBCP (P<0.05), and soil physical and chemical properties showed a significant positive correlation with enzyme activities (P<0.05). Soil microbial biomass in ungrazed alpine meadows showed a significant positive effect on MBCP (P<0.01); soil physicochemical properties were positively correlated with MBCP, and enzyme activity was negatively correlated with MBCP; soil physicochemical properties indirectly affected MBCP through enzyme activity and microbial biomass, and enzyme activity indirectly affected MBCP through microbial biomass and soil physicochemical properties (Fig. 6a)). Soil microbial biomass in lightly and moderately grazed alpine meadows showed a significant positive correlation (P<0.01) with MBCP; enzyme activity showed a positive correlation with MBCP, while at the same time, enzyme activity affected MBCP indirectly through soil microbial biomass and soil physicochemical properties, respectively (Fig. 6(b and c)).
Discussion
Effects of Litter Inputs on Soil Physicochemical and Enzymatic Activities of Alpine Meadow
In this study, we found that ungrazed, lightly grazed, and moderately grazed alpine meadow soil NH4⁺-N and NO3--N showed an overall trend of gradual increase under litter inputs, of which lightly grazed was higher than that of ungrazed and moderately grazed, and both peaked at T3, with the maxima of 24.89 mg/kg and 0.86 mg/kg, respectively. Soil bulk weight showed a trend of gradual decrease; SM, EC, and pH did not have a uniform pattern of change under litter inputs, and the differences were significant (P<0.05). This is consistent with the results of existing studies [33]. Litter inputs are a major pathway for soil material cycling and energy flow, affecting the supply of carbon sources to soil microorganisms and changes in soil enzyme activities [34]. It has been shown that changes in litter inputs affect the microenvironment and enzyme activities by altering the soil environment, organic carbon content, and soil nutrients [35]. This study found that S-β-XYS, S-β-GC, S-FDA, S-DHA, and CBH showed a gradual increase with increasing litter inputs, and all had maximum values at T3. The values of S-β-XYS, S-β-GC, GOD, and S-DHA were higher than those of the ungrazed and moderately grazed under lightly grazing, and the S-β-XYS, S-β-GC, and S-DHA had maximum values of 16.87 U/g, 41.09 U/g, and 21.01 U/g at T3, respectively (Fig. 2(a, b, and e)). This is similar to the existing study [33]. This may be because litter is an important carbon source for microorganisms, increasing the available organic matter content in the soil. The input of new carbon sources may trigger the “initiation effect” of carbon, leading to the decomposition of existing soil organic matter [36], which requires the synergistic action of multiple enzymes, resulting in a significant increase in soil enzyme activities in the short term. At the same time, microbial adaptive regulation drives soil microorganisms to adapt to new environments by modulating their enzyme synthesis strategies in response to resource changes.
Effect of Litter inputs on MBC, MBN, and MBC/MBN in Alpine Meadow
Soil microbial biomass is an important parameter in the assessment of soil active nutrient pools, and its transformation is rapid and sensitive, playing an important role in driving the biogeochemical cycling of soil carbon (C) and nitrogen (N) elements [37]. It not only reflects the activity of soil microorganisms but also affects soil fertility and ecosystem function. The results of this study showed that the soil MBC and MBN in ungrazed, lightly grazed, and moderately grazed alpine meadows were positively affected by litter inputs, which all peaked under T3 treatment, which is consistent with the existing studies [9, 13]. Because soil microbial biomass is positively correlated with increases in litter inputs in nutrient-limited areas (Fig. 3a) and b)), most soil microbes, including bacteria and fungi, rely on the decomposition of litter materials for energy and nutrients [38]. Litter matter serves as an important carbon source for microorganisms in grassland ecosystems. When litter is input into an alpine meadow, the organic matter in it is decomposed by microorganisms, thus releasing carbon for microbial utilization, which in turn increases the MBC in the soil. The value of MBC/MBN can be used as an important indicator for determining the nutrient limitation of the soil [39]. The present study found that the ungrazed and moderately grazed MBC/MBN values showed a dynamic trend of gradual decrease with the increase of litter, which is similar to the existing study [40]. Changes in the MBC/MBN ratio reflected the process of nitrogen mineralization and fixation in the soil. This may be because the new carbon source input improved soil nitrogen effectiveness and promoted nitrogen assimilation by microorganisms, leading to an increase in MBN. Meanwhile, litter inputs may affect the structure and function of alpine meadow ecosystems through a feedback mechanism driven by structural adjustment of soil microbial communities, increased nitrogen effectiveness, and changes in the soil environment.
Effect of Litter Inputs on Soil MBCP in Alpine Meadow
MBCP is the sum of carbon contained in the bodies of all microorganisms (including bacteria, fungi, actinomycetes, protozoa, and algae) in the soil. In this study, it was found that there was no significant positive or negative effect of MBCP with litter inputs, which is similar to the existing study [41]. The positive feedback loop of plant-microbe interactions in terrestrial ecosystems contributes to nutrient exchange, which is manifested in alpine meadows as “nitrogen promotes nitrogen fixation-carbon promotes nitrogen retention”. Plants provide carbon to microorganisms through root secretion, microorganisms provide directly available nitrogen to plants through mineralization, and root secretion regulates MBCP [42]. Meanwhile, the low temperature, low decomposition rate, and low enzyme activity of alpine meadows in the Sanjiangyuan area may largely affect MBCP. It may be because the unique ecosystem of alpine meadows affects the soil microbial community organization and the normal expression of functional genes, and the lag effect of soil leads to the inability to observe the response of MBCP to litter in a short period of time.
The content of MBCP in soil varies according to the type of grassland, climatic conditions, soil properties, the process of soil microbial synthesis and metabolism, etc. The present study did not explore the response of MBC and MBCP to meteorological factors, the regulatory mechanisms of soil factors, and microbial characteristics on MBC and MBCP, which is a limitation of this study. Subsequent studies should combine meteorological and soil factors to analyze the MBC and MBCP regulatory mechanisms.
Mechanisms of Soil Physicochemical and Enzyme Activities Affecting MBCP
This study found significant correlations between soil physicochemical properties, enzyme activities, and microbial biomass in alpine meadows (Fig. 5 (a-c)). Structural equation modeling indicated that soil physicochemical properties and enzyme activities. Soil microbial biomass and MBCP all showed significant positive correlations (P<0.05) (Fig. 5(a-c)). This may be due to the role of inter-root effects of alpine meadow plants. Plant inter-root secretions (which change soil pH and release organic carbon bound to minerals) promote microbial decomposition, which increases MBCP [43]. The physicochemical properties of ungrazed and lightly grazed alpine meadow soils showed a positive correlation with MBCP, but the difference was not significant (P>0.05). This may be because both ungrazed alpine meadow soil physicochemical properties (ST, SM, EC, PH, and BD) and lightly grazed soil physicochemical properties (ST, SM, EC, PH, BD, NH₄⁺-N, and NO₃⁻-N) did not show significant correlation with MBCP. This is because conventional structural equation modeling is used to test complex causal relationships between variables. In this study, the bias introduced by nested data was corrected by mixed-effects modeling to improve the estimation accuracy of SEM [44].
Due to the perennial low temperature and low decomposition rate on the Tibetan Plateau, soil organic matter decomposition and deep carbon pool dynamics need long-term monitoring to show significant trends, resulting in the lag effect of nutrient cycling in alpine meadow ecosystems not being fully considered. The short experimental period of this study is a limitation. We should carry out long-term localization experiments to explore the synergistic effects of litter inputs on enzyme activities and soil carbon sinks under the background of climate change. To explore the decomposition period of litter materials and the series of reactions and biochemical processes involved in the decomposition of litter materials, the microbial genetic mechanism of the changes in enzyme activity can be analyzed by combining it with macrogenomics technology.
Conclusions
With the increase of litter input, soil S-β-XYS, S-β-GC, S-FDA, S-DHA, CBH, MBC, MBN content, and MBCP had maximum values at T3, and the values of S-β-XYS, S-β-GC, GOD, S-DHA, and MBCP were higher than those of the ungrazed and moderately grazed under light grazing. Structural equation modeling showed that soil microbial biomass of ungrazed, lightly grazed, and moderately grazed alpine meadows was significantly positively correlated with MBCP, and ungrazed enzyme activities were negatively correlated with MBCP; soil enzyme activities of lightly and moderately grazed alpine meadows were positively correlated with MBCP. The results of this study provide scientific guidance for the study of carbon pools in the Tibetan Plateau. Follow-up studies can be carried out for long-term monitoring to systematically analyze the effect of microbial biomass carbon pools in alpine meadows on litter inputs under global climate change.

