Introduction
Potatoes are recognized as the fourth major global food crop [1]. It has a long planting history and comprises several varieties. It is one of China’s most important economic crops. Long-term continuous planting of potatoes has re-sulted in a severe imbalance of soil microbial communities, a high incidence of soil-borne diseases, and a severe decline in yield [2, 3].
Soil microorganisms play a key role in the ecosystem [4] and are important factors related to soil quality [5], soil fertility, and productivity [6]. Changes in soil microorganisms influence the absorption and transformation of soil nutrients [7]. Therefore, the number and types of soil microorganisms may affect plant growth, development, and health [8, 9]. In recent years, several studies have shown that continuous cropping has led to the imbalance and diversity of soil microbial communities [10, 11]. Continuous cropping facilitates a significant increase in plant fungal pathogens in soil while the abundance of beneficial bacteria and actinomycetes decreases [12, 13]. Continuous planting of potatoes significantly reduces the diversity of soil bacterial communities and the abundance of beneficial bacteria [14, 15]. For example, the abundance of beneficial fungi such as Chaetomium decreases, whereas that of harmful fungi such as Verticillium, Fusarium, and Col-letotrichum increases. It is essential enzyme activity for bacterial activities.
Crop rotation is considered an effective way to mitigate the adverse effects of continuous cropping [16]. It improves the physical and chemical properties of soil and enhances soil fertility [17, 18]. Crop rotation can also significantly increase the abundance and diversity of soil microbial communities [19]. For example, wheat-canola [20] and corn-soybean [21] crop rotation significantly impacts soil microbial communities, and the rotation of different crops and cucumbers improves the uniformity of the soil microbial community and the soil microecological environment [22]. Although several studies have focused on the effects of crop rotation on potato quality and disease occurrence [23, 24], the effects of rye-potato rotation on potato physical features, soil physical and chemical properties, and microbial community structure have not been studied.
The aim was to study the effects of rye-potato rotation on soil physical and chemical properties and soil microbial community structure and to provide a theoretical basis for reducing obstacles to continuous potato cropping.
Materials and Methods
Field Experiment
The experiment was conducted at the planting base of Chunhua Potato Planting Co., Ltd., Erdaoqu Town-ship, Wuyuan County, Zhangjiakou City, Hebei Province, China. The latitude and longitude of the area are 114°50′–116°04′E, 41°14′–41°57′N, situated in the southern margin of the Inner Mongolia Plateau. The soil type is chestnut clay. The nitrogen content accounts for 0.5% to 0.8% of dry matter, up to 2.2%, and the ash element reaches 6% to 16%, mainly potassium and calcium. Generally, the calcium layer of chestnut soil is deep and thick, with a lime content of up to 10% to 30%, with the highest being up to 40% and the lowest being less than 5%. The soil is alkaline and light in texture. The average elevation is 1,536 m, and the climate is a temperate continental grassland climate. The average temperature during the growth cycle is 9℃, and the an-nual precipitation is 426 mm.
Potatoes have been planted for six consecutive years in the continuous experimental field. Rye and potatoes have been planted in rotation for 6 years in the rye-potato rotation field. Over the past six years, the use of pesticides, fertilizers, plastic film mulching, and the amount of water used for farming and irrigation have been the same in both rye-potato rotation fields and potato continuous cropping. Varieties of potatoes include Favorita (a virus-free potato variety). In the continuous cropping field, the basic physical and chemical properties of the experimental field are 51.24 mg/kg of alkaline nitrogen, 42.47 mg/kg of available phosphorus, 290.00 mg/kg of available potassium, 10.99 g/kg of organic matter, and a pH of 6.12 (water:soil 2.5:1). In the crop rotation field, potatoes and rye were rotated every other year. The basic physical and chemical properties of the experimental field were 61.77 mg/kg alkali nitrogen, 11.00 mg/kg available phosphorus, 82.57 mg/kg available potassium, 15.61 g/kg organic matter, and a pH of 7.14 (water:soil 2.5:1).
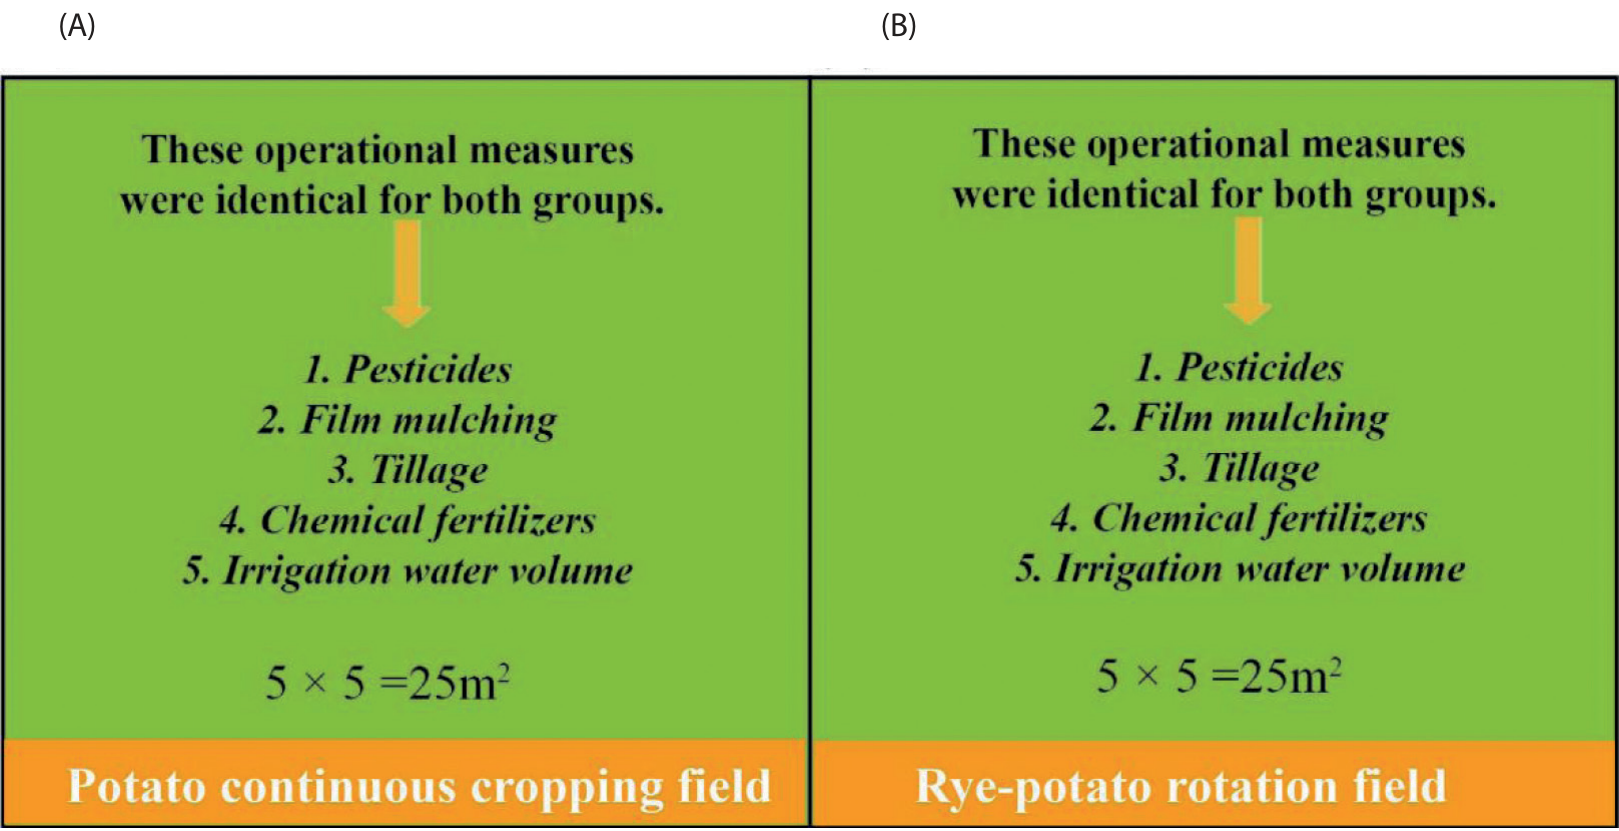
The field experiment adopted a random block design, and three plots were set for continuous cropping and rotation. The plot area was 5 × 5 = 25 m2, plant spacing was 20 cm, and row spacing was 60 cm (Fig. S1). The rest of the conditions, including the application of pesticides, chemical fertilizers, film mulching, tillage, and irrigation water volume, are all in accordance with local customs, and the measures for both groups are the same.
All the soil samples were collected in 2018. Sampling was performed during five periods: before sowing (May 1st), seedling period (June 25th), flowering period (July 28), maturity period (August 25th), and after-harvest period (September 15th). A five-point sampling method was used for each period, and soil samples with a depth of 5-20 cm were collected at five points before sowing and after harvesting. In the seedling, flowering, and maturity periods, soil samples were collected from the potato root zone. Soil samples were evenly mixed together into one sample, collected into a Ziplocka bag, and stored directly frozen at −80°C until DNA extraction [25].
Determination of Potato Physical Features
During the harvest, potatoes from the SC and RC groups were collected using a five-point sampling method. Initially, the soil on the surface of the potatoes was washed away with clean water. Subsequently, a visual inspection method was employed to observe the physical features of the potatoes, including whether the skin was smooth and the potato buds were deep or shallow [26].
Determination of Soil Physical and Chemical Properties
Soil samples were air-dried and passed through a 2-mm aperture sieve. Soil pH was determined with a compound electrode (Mp521 Lab pH meter, Japan) at a soil:water ratio of 1:2.5 (w/v; g·cm-3). Soil available phosphorus (AP) and available potassium (AK) were determined, and soil alkaline nitrogen was assessed using an alkaline hydrolysis diffusion method [27, 28]. Soil organic matter (OM) was determined using the oil bath heating-potassium dichro-mate (K2Cr2O7) volumetric method. Briefly, the temperature of the oil bath was 180°C, it was boiled for 5 min, a 0.4 mol/L K2Cr2O7-H2SO4 solution was used to oxidize the organic matter in the soil, and the remaining K2Cr2O7 was used in FeSO4 for titration. Each soil sample was measured in triplicate.
Determination of Soil Biological Indicators
Soil enzymes were determined using kits for soil urease activity detection, soil sucrase activity detection, and soil acid phosphatase activity detection (Solarbio Technology Co. Ltd., China), following the manufacturer’s instructions [29]. The extraction of each soil sample was repeated three times.
DNA Extraction
Total genomic DNA was extracted from the samples using the CTAB method. DNA concentration and purity were measured on a 1% agarose gel using the M5 Gel Extraction Kit (Mei5 Biotechnology Co., Ltd). According to the concentration, DNA was diluted to 1 ng/μL using sterile water.
PCR Amplification and Sequencing
PCR amplification of the bacterial 16S rRNA gene V3–V4 region was performed using the forward primer 338F (5’-ACTCCTACGGGAGGCAGCA-3’) and the reverse primer 806R (5’-GGACTACHVGGGT-WTCTAAT-3’). For amplification of fungal IT sequences, the forward primer ITS5F (5’-GGAAGTAAAA-GTCGTAACAAGG-3’) and the reverse primer ITS1R (5’-GCTGCGTTCTTCATCGATGC-3’) were used. All PCR reactions were conducted in 30-μL reactions with 15 μL of Phusion® High-Fidelity PCR Master Mix (Bio-lab Technology Co., Ltd., China), 0.2 μM of the forward and reverse primers, and about 10 ng of template DNA. Thermal cycling consisted of an initial denaturation at 98°C for 1 min, followed by 30 cycles of denaturation at 98°C for 10 s, annealing at 50°C for 30 s, elongation at 72°C for 30 s, and a final 72°C for 5 min. Sequencing libraries were generated using Ion Plus Fragment Library Kit 48 reactions (Thermo Fisher Scientific Co., Ltd., USA) following the manufacturer’s recommendations [30]. Library quality was assessed on the Qubit@2.0 Fluorometer (Thermo Fisher Scientific Co., Ltd., USA). Finally, the library was sequenced on an Ion S5TM XL platform, and 600-bp single-end reads were generated.
Statistical Analysis
Sequence analysis was performed using Uparse (v7.0.1001, http://drive5.com/uparse/) [31]. Sequences with ≥ 97% similarity were assigned to the same OTU. Alpha diversity was applied in analyzing the species diversity of samples, and the Chao l, Shannon, and Good-coverage indices of our samples were calculated with QIIME (Version1.7.0) and displayed with R software (Version. 2.15.3) [32]. Beta diversity on both weighted and unweighted unifrac was calculated by QIIME software (ver. 1.7.0). The results for both groups were analyzed with a single factor ANOVA. Statistical analysis of the data was performed in IBM SPSS 25.0 software, and statistical significance was considered at P < 0.05. Origin Pro 2018 was used for mapping.
Results
Potato Physical Features
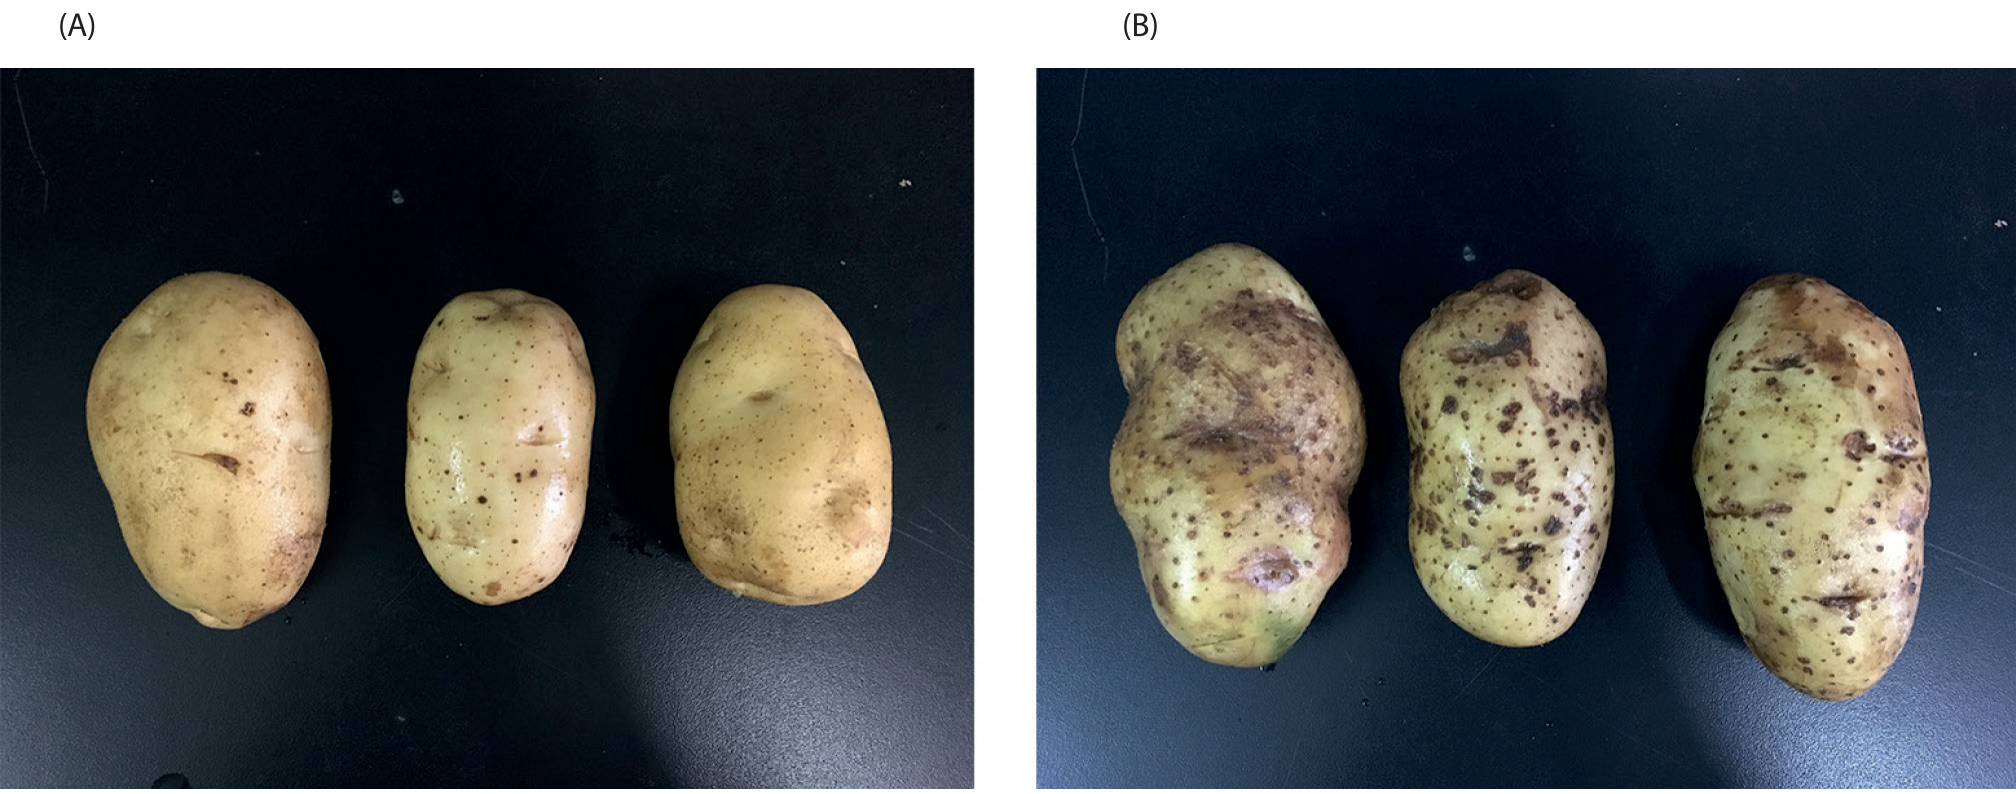
The potatoes in the rye-potato rotation crop (RC) group field had smooth skin, small spots, and shallow buds (Fig. 1A), whereas those in the continuous cropping field (SC) group had many rough spots and deep buds (Fig. 1B). During the harvesting process, potatoes in the rotation field were easier to collect than in the continuous field, which may be related to changes in soil physical and chemical properties in the rotation and continuous cropping fields.
Soil Physical and Chemical Properties and Soil Enzyme Activity
Table 1 shows that the content of soil organic matter (OM) was significantly higher in the RC group than the SC group at all five periods (before sowing (P = 0.016, percentage = 42.04%), seedling (P = 0.0003, percentage = 65.36%), flowering (P = 0.044, percentage = 55.91%), maturity (P = 0.002, percentage = 66.85%), and after-harvest (P = 0.033, percentage = 53.91%) periods). The alkaline nitrogen (AN) content in the RC group was also significantly higher than the SC group during the five periods (before sowing: P = 0.003, seedling: P = 0.014, flowering: P = 0.003, maturity: P = 0.008, after-harvest: P = 0.031), and increased by 36.39% at the seedling period and 42.29% at after harvest. The pH of the RC group was significantly higher than the SC group during the four periods (before sowing: P = 0.008, seedling: P = 0.027, flowering: P = 0.0001, and after-harvest: P = 0.002), except for the maturity period.
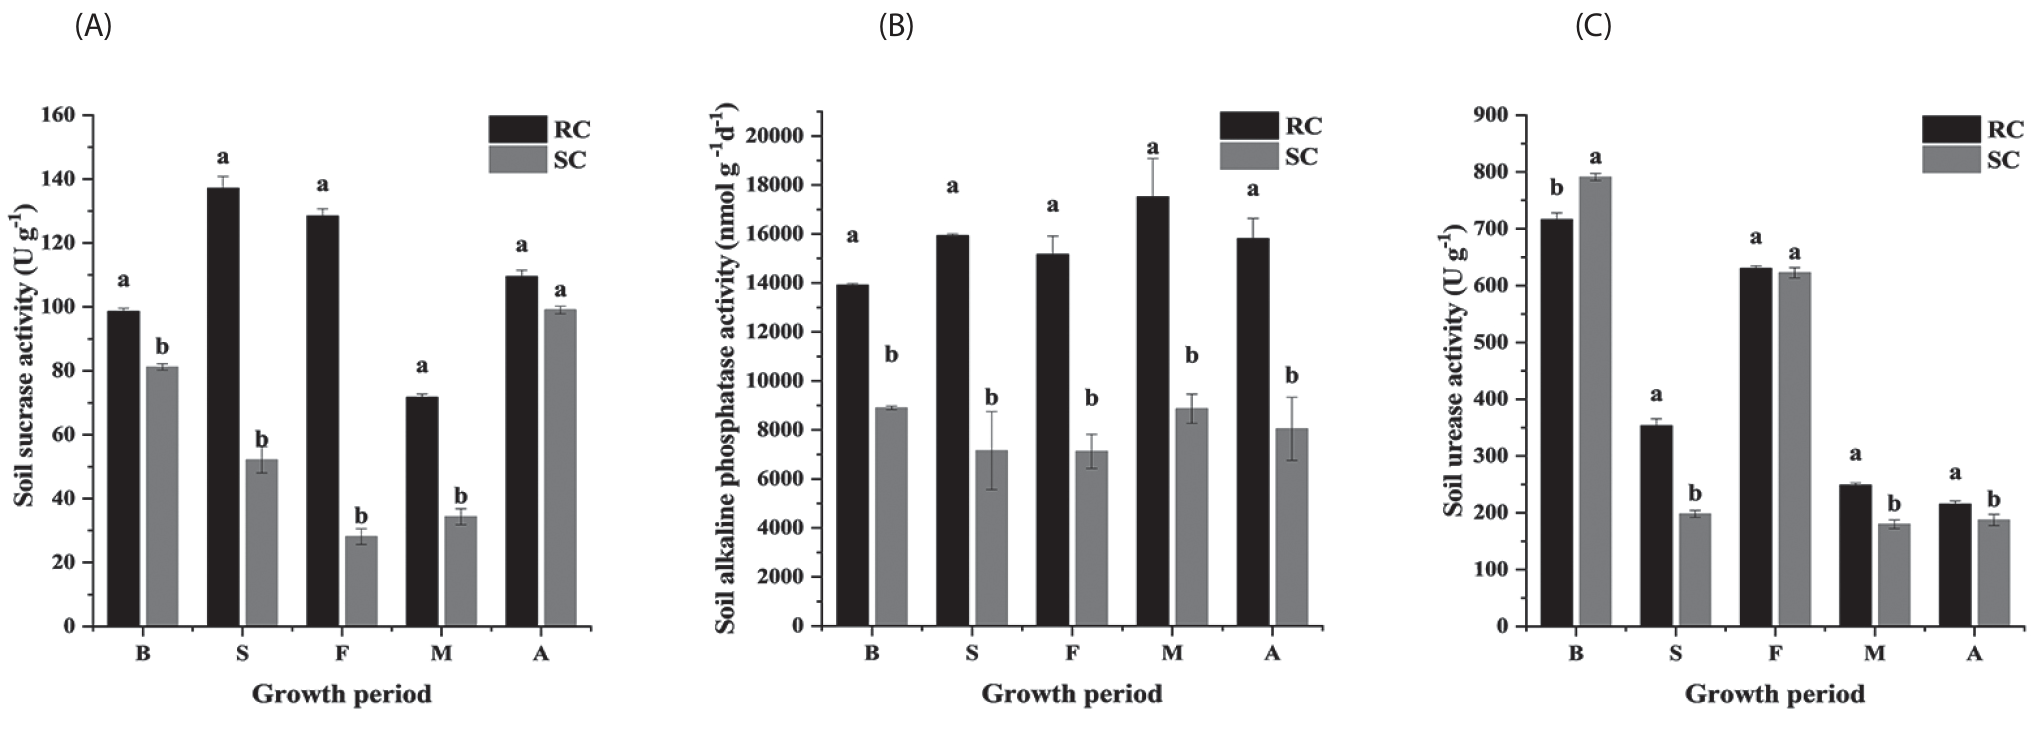
Fig. 2 shows the soil enzyme activity at each period. Compared with the SC group, soil alkaline phosphatase activity in the RC group significantly (P = 0.000, P = 0.001, P = 0.0003, P = 0.002, P = 0.003) increased during sowing, seedling, flowering, maturity, and after-harvest periods. Alkaline phosphatase activity was the highest at the seedling and flowering periods, which increased by 1.23-fold and 1.13-fold, respectively. Soil sucrase significantly increased by 1.63-fold, 3.58-fold, and 1.09-fold in the seedling, flowering, and maturity periods, respectively. Soil urease significantly (P = 0.000, P = 0.000, P = 0.024) increased by 78%, 38%, and 15% during the seedling period, maturity period, and after-harvest periods. Soil sucrase and alkaline phosphatase in the RC group were at their highest during the seedling and flowering periods.
Soil Microbial Diversity
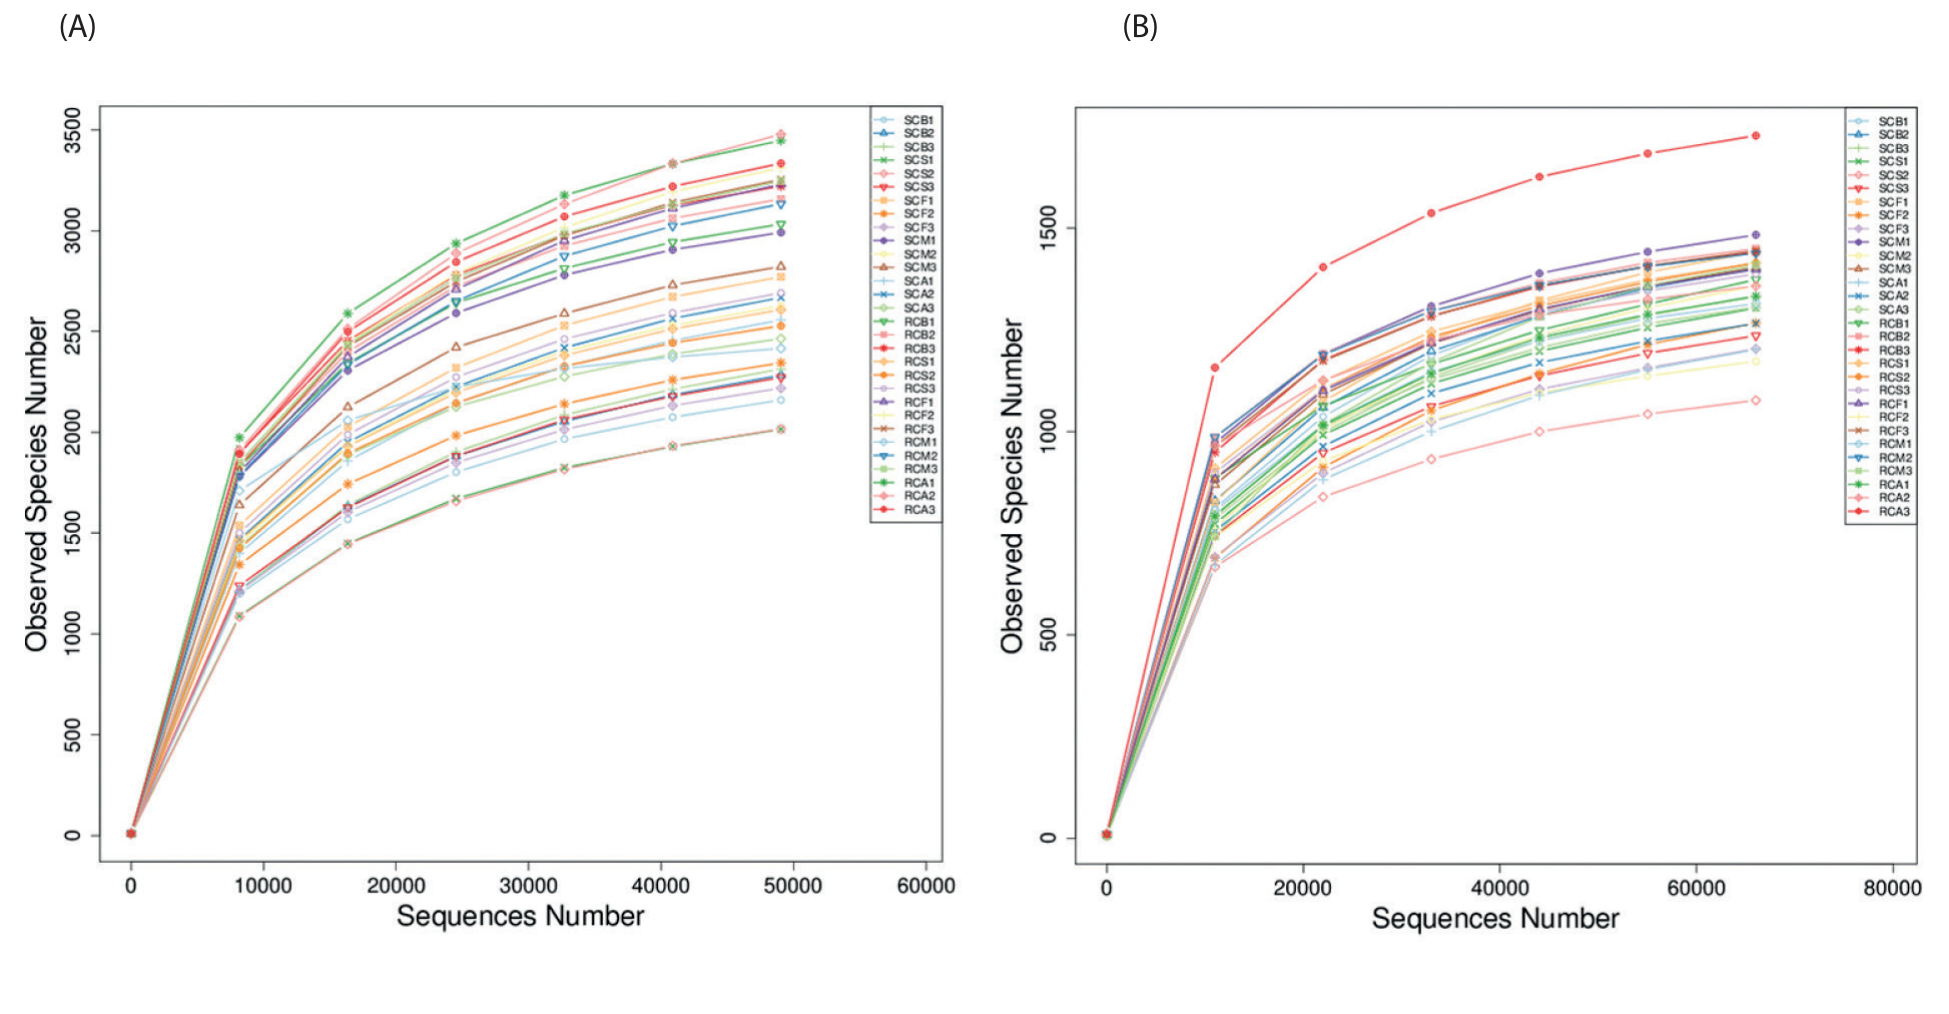
The rarefaction curve of each sample for the high-throughput sequencing was close to the saturation plateau (Fig. S2), indicating that the sequencing library had reached saturation and that the results truly reflected the sample conditions. The sequencing results for bacteria are shown in Table 2. The coverage of all samples was > 97.6%, and the effective read range for each sample was 75,706– 86,874. The OTU of each sample ranged from 2,411 to 3,676. The Shannon indices of the RC group were significantly (P = 0.000, P = 0.004, P = 0.003, P = 0.001, P = 0.001) higher than those of the SC group before sowing, seedling, flowering, maturity, and after-harvest periods. The Chao 1 indices of the RC group were significantly (P = 0.022, P = 0.036, P = 0.019, P = 0.042) higher than the SC group at before sowing, seedling, flowering, and after-harvest periods. These results showed that the RC group improved bacterial diversity.
Table 1.
Physical and chemical properties of soil.
[i] Notes: SCB, SCS, SCF, SCM, and SCA represent before sowing, seedling, flowering, maturity, and after-harvest periods of continuous potato cropping, respectively. RCB, RCS, RCF, RCM, and RCA represent before sowing, seedling, flowering, maturity, and after-harvest periods of the rye-potato crop rotation, respectively. Abbreviations: OM, Organic matter; AN, alkaline nitrogen; AP, Available P; AK, Available K. Data are the mean±standard error (n = 3) and within each column; different letters indicate significant differences (P < 0.05).
Fig. 2.
Analysis of different planting methods on soil enzyme activity. (A) Soil sucrase activity; (B) Soil alkaline phosphatase activity; (C) Soil urease activity. RC and SC represent rye-potato crop rotation and continuous potato cropping, respectively. B, S, F, M, and A represent before sowing, seedling, flowering, maturity, and after-harvest periods, respectively. Different letters indicate significant differences (P < 0.05).
The sequencing coverage of fungi in all samples was > 99.4% (Table 3). The effective read range for each sample was 80,080–80,709. The OTUs of each sample ranged from 1,357 to 1,620. The Shannon index of the RC group was significantly (P = 0.017, P = 0.014, P = 0.011) higher than the SC group in the periods before sowing, seedling, and after-harvest. Chao1 in the RC group in the whole sampling period was also higher than the SC group. There were significant (P = 0.009, P = 0.046, P = 0.0369) differences among the seedling, flowering periods, and after-harvest periods. The results showed that the RC group increased soil fungal diversity.
Table 2.
Diversity of soil bacterial communities.
[i] Notes: SCB, SCS, SCF, SCM, and SCA represent before sowing, seedling, flowering, maturity, and after-harvest periods of continuous potato cropping, respectively. RCB, RCS, RCF, RCM, and RCA represent before sowing, seedling, flowering, maturity, and after-harvest periods of the rye-potato crop rotation, respectively. Reads: the optimized sequences; OTU, operational taxonomic unit. The numbers within parentheses are the lower and upper limits in the statistical analysis of the corresponding data, respectively.
Table 3.
Diversity of soil fungal communities.
[i] Notes: SCB, SCS, SCF, SCM, and SCA represent the before sowing, seedling, flowering, maturity, and after-harvest periods of continuous potato cropping, respectively. RCB, RCS, RCF, RCM, and RCA represent before sowing, seedling, flowering, maturity, and after-harvest periods of the rye-potato crop rotation, respectively. Reads: the optimized sequences; OTU, operational taxonomic unit. The numbers within parentheses are the lower and upper limits in the statistical analysis of the corresponding data, respectively.
Venn analysis showed that the number of bacterial OTUs shared by each sampling period in the SC and RC groups was 1,318 (Fig. 3A). Except for the flowering and maturity periods, the unique OTU number of the RC group was higher than the SC group. The number of shared fungal OTUs in all periods was 607 (Fig. 3B). The number of OTUs in the RC group was higher than that of the SC group in all periods, which coincided with the changes in total OTUs. There were various numbers of shared and unique OTUs among samples, suggesting that although the soil microorganisms of continuous cropping and rotation had similar species, these had different community structures.
Soil Microbial Composition
With continuous cropping and rotation of potatoes, Proteobacteria, Bactercidetes, Actinobacteria, Firmicutes, Acidobacteria, Gemmatimonadetes, Chloroflexi, unidentified bacteria, Verrucomicrobia, and Fusobacteria were the 10 predominant bacterial phyla (Fig. 4A). Compared with the SC group, the relative abundance of bacteria in the phyla level of the RC group differed. The relative abundance of Acidobacteria significantly increased (P = 0.006, P = 0.020, P = 0.007, P = 0.019, P = 0.002 ) in the five periods by 258.86%, 51.93%, 125.48%, 64.22%, and 84.65%. The relative abundance of Actinobacteria increased by 9.43%, 12.38%, 25.22%, 23.61%, and 35.83% among these five periods, with significant differences (P = 0.018, P = 0.034, P = 0.031) among the flowering, maturity, and after-harvest periods. The relative abundance of Firmicutes significantly (P = 0.021) increased by 37.62% during the maturity period. The relative abundance of Chloroflexi significantly increased (P = 0.033, P = 0.019 ) by 38.63% and 65.16% during the seedling and after-harvest periods respectively.
Fig. 3.
Venn analysis of OTUs of bacterial and fungal communities. (A) Bacteria; (B) Fungi. SCB, SCS, SCF, SCM, and SCA represent before sowing, seedling, flowering, maturity, and after-harvest periods of continuous potato cropping, respectively. RCB, RCS, RCF, RCM, and RCA represent before sowing, seedling, flowering, maturity, and after-harvest periods of the rye-potato crop rotation, respectively.
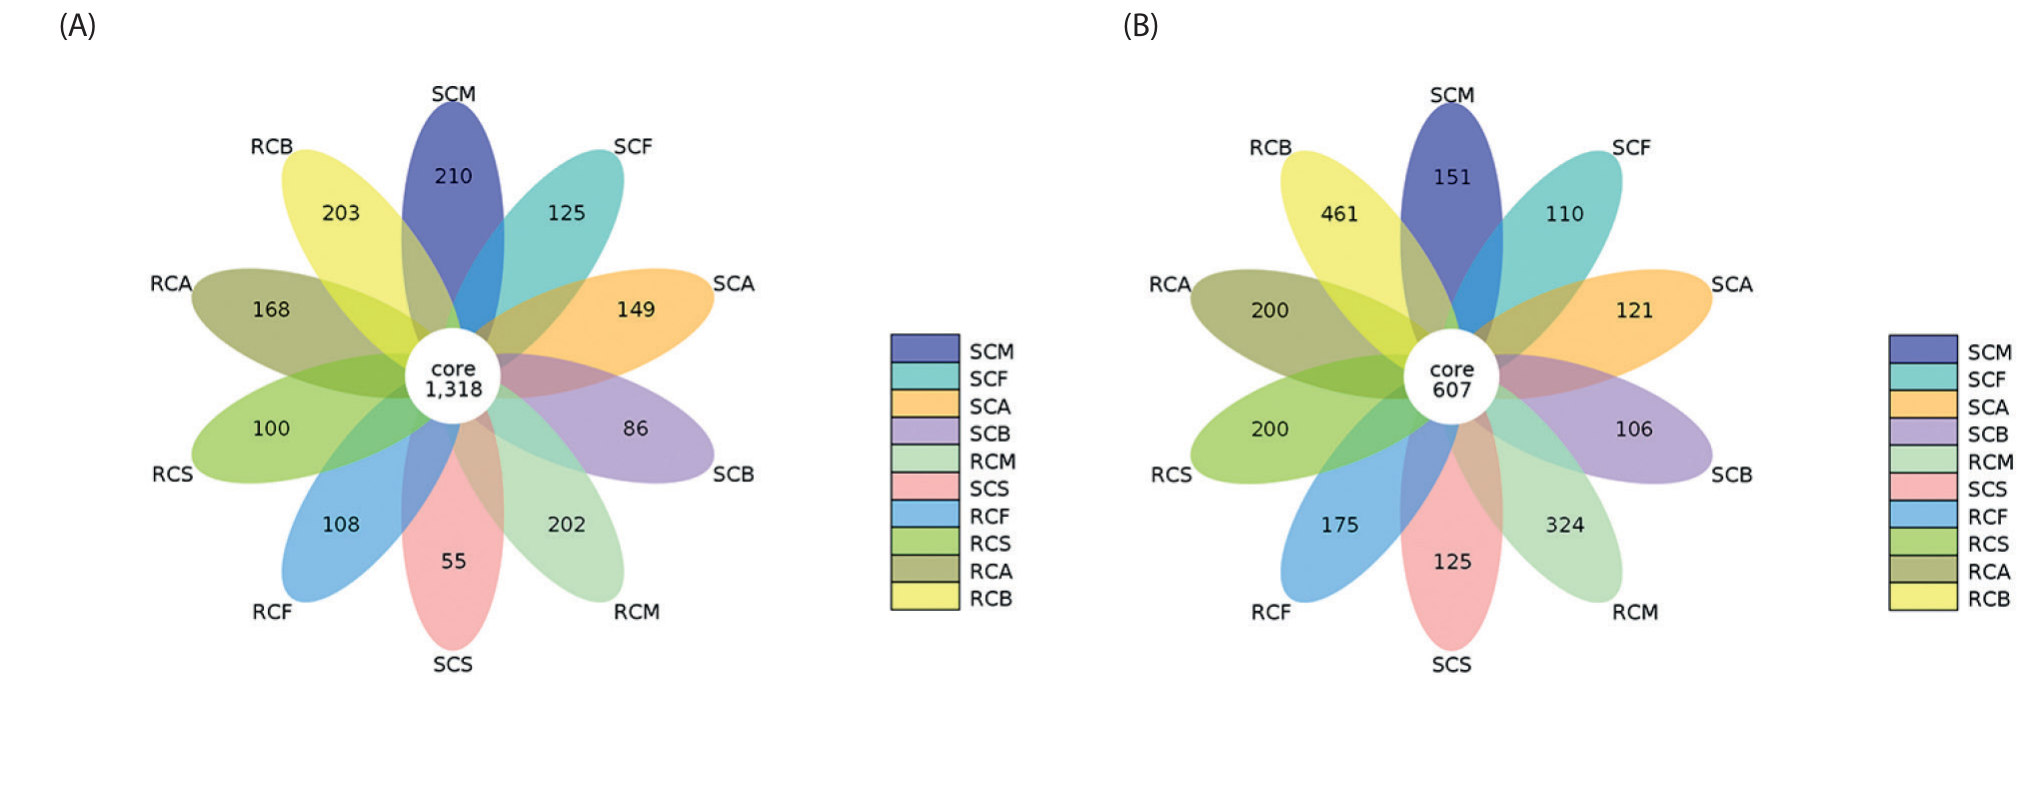
Fig. 4.
Analysis of soil microbial at the phylum level. (A) Bacteria; (B) Fungi. SCB, SCS, SCF, SCM, and SCA represent before sowing, seedling, flowering, maturity, and after-harvest periods of continuous potato cropping, respectively. RCB, RCS, RCF, RCM, and RCA represent before sowing, seedling, flowering, maturity, and after-harvest periods of the rye-potato crop rotation, respectively.
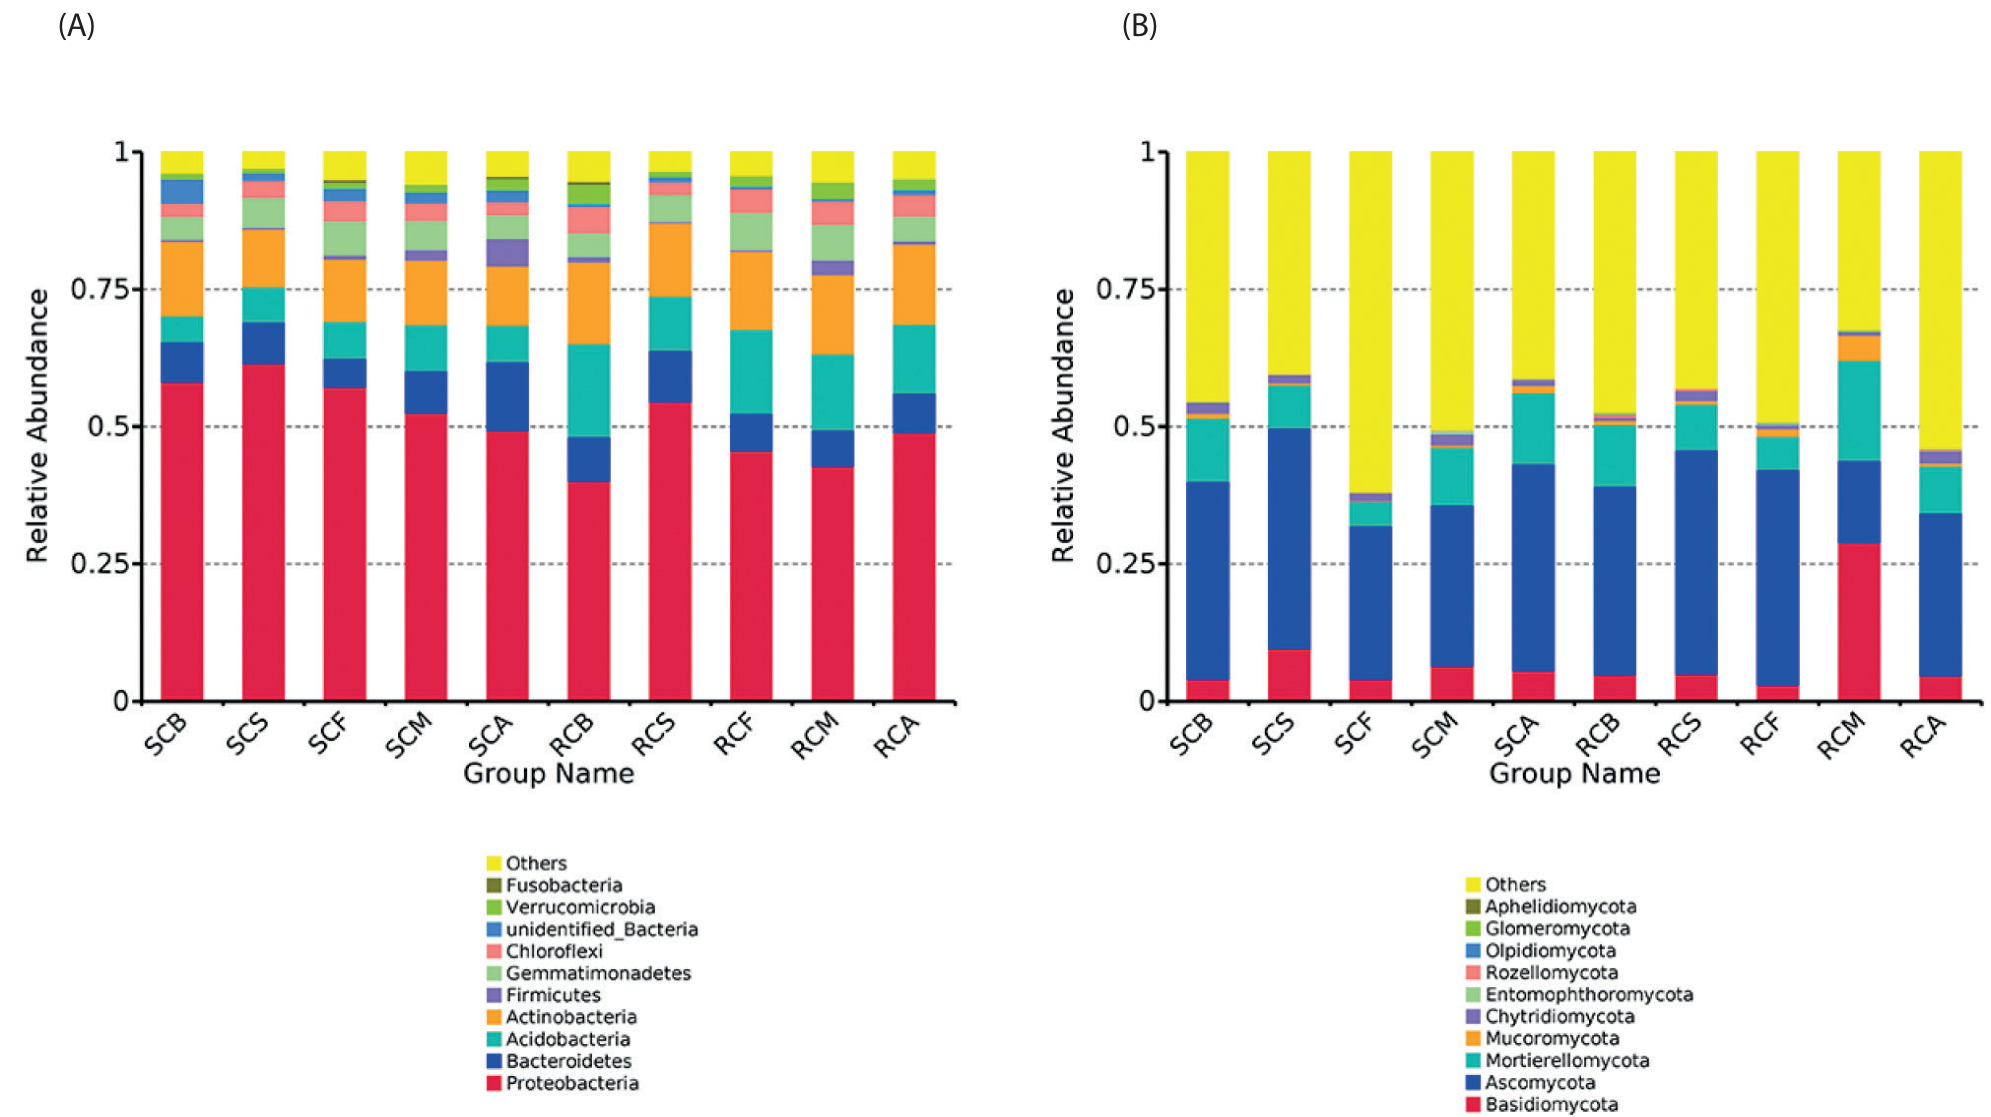
For fungi, Basidiomycota, Ascomycota, Mortierellomy-cota, Mucoromycota, Chytridiomycota, Entomophthoro-mycota, Rozellomycota, Olpidiomycota, Glomeromycota, and Aphelidiomycota were the predominant phyla across all periods (Fig. 4B, Table S1). Among these, Ascomycota has the highest abundance, followed by Basidiomycota. It shows that in this experimental field, the main pathogenic bacteria that can cause potato diseases are Ascomycota and Basidiomycota. Compared with the SC group, the relative abundance of Ascomycota in the RC group significantly (P = 0.000, P = 0.000) decreased by 49.26% and 21.24% in the maturity and after-harvest periods, respectively, and peaked during the seedling period in the RC group and the SC group, then subsequently decreased. The relative abundance of Basidiomycota decreased by 47.97% in the seedling period but increased by 344.17% in the maturity period.
Fig. 5.
Analysis of soil microbial at the genus level. (A, C) Bacteria; (B, D) Fungi. SCB, SCS, SCF, SCM, and SCA represent before sowing, seedling, flowering, maturity, and after-harvest periods of continuous potato cropping, respectively. RCB, RCS, RCF, RCM, and RCA represent before sowing, seedling, flowering, maturity, and after-harvest periods of the rye-potato crop rotation, respectively.
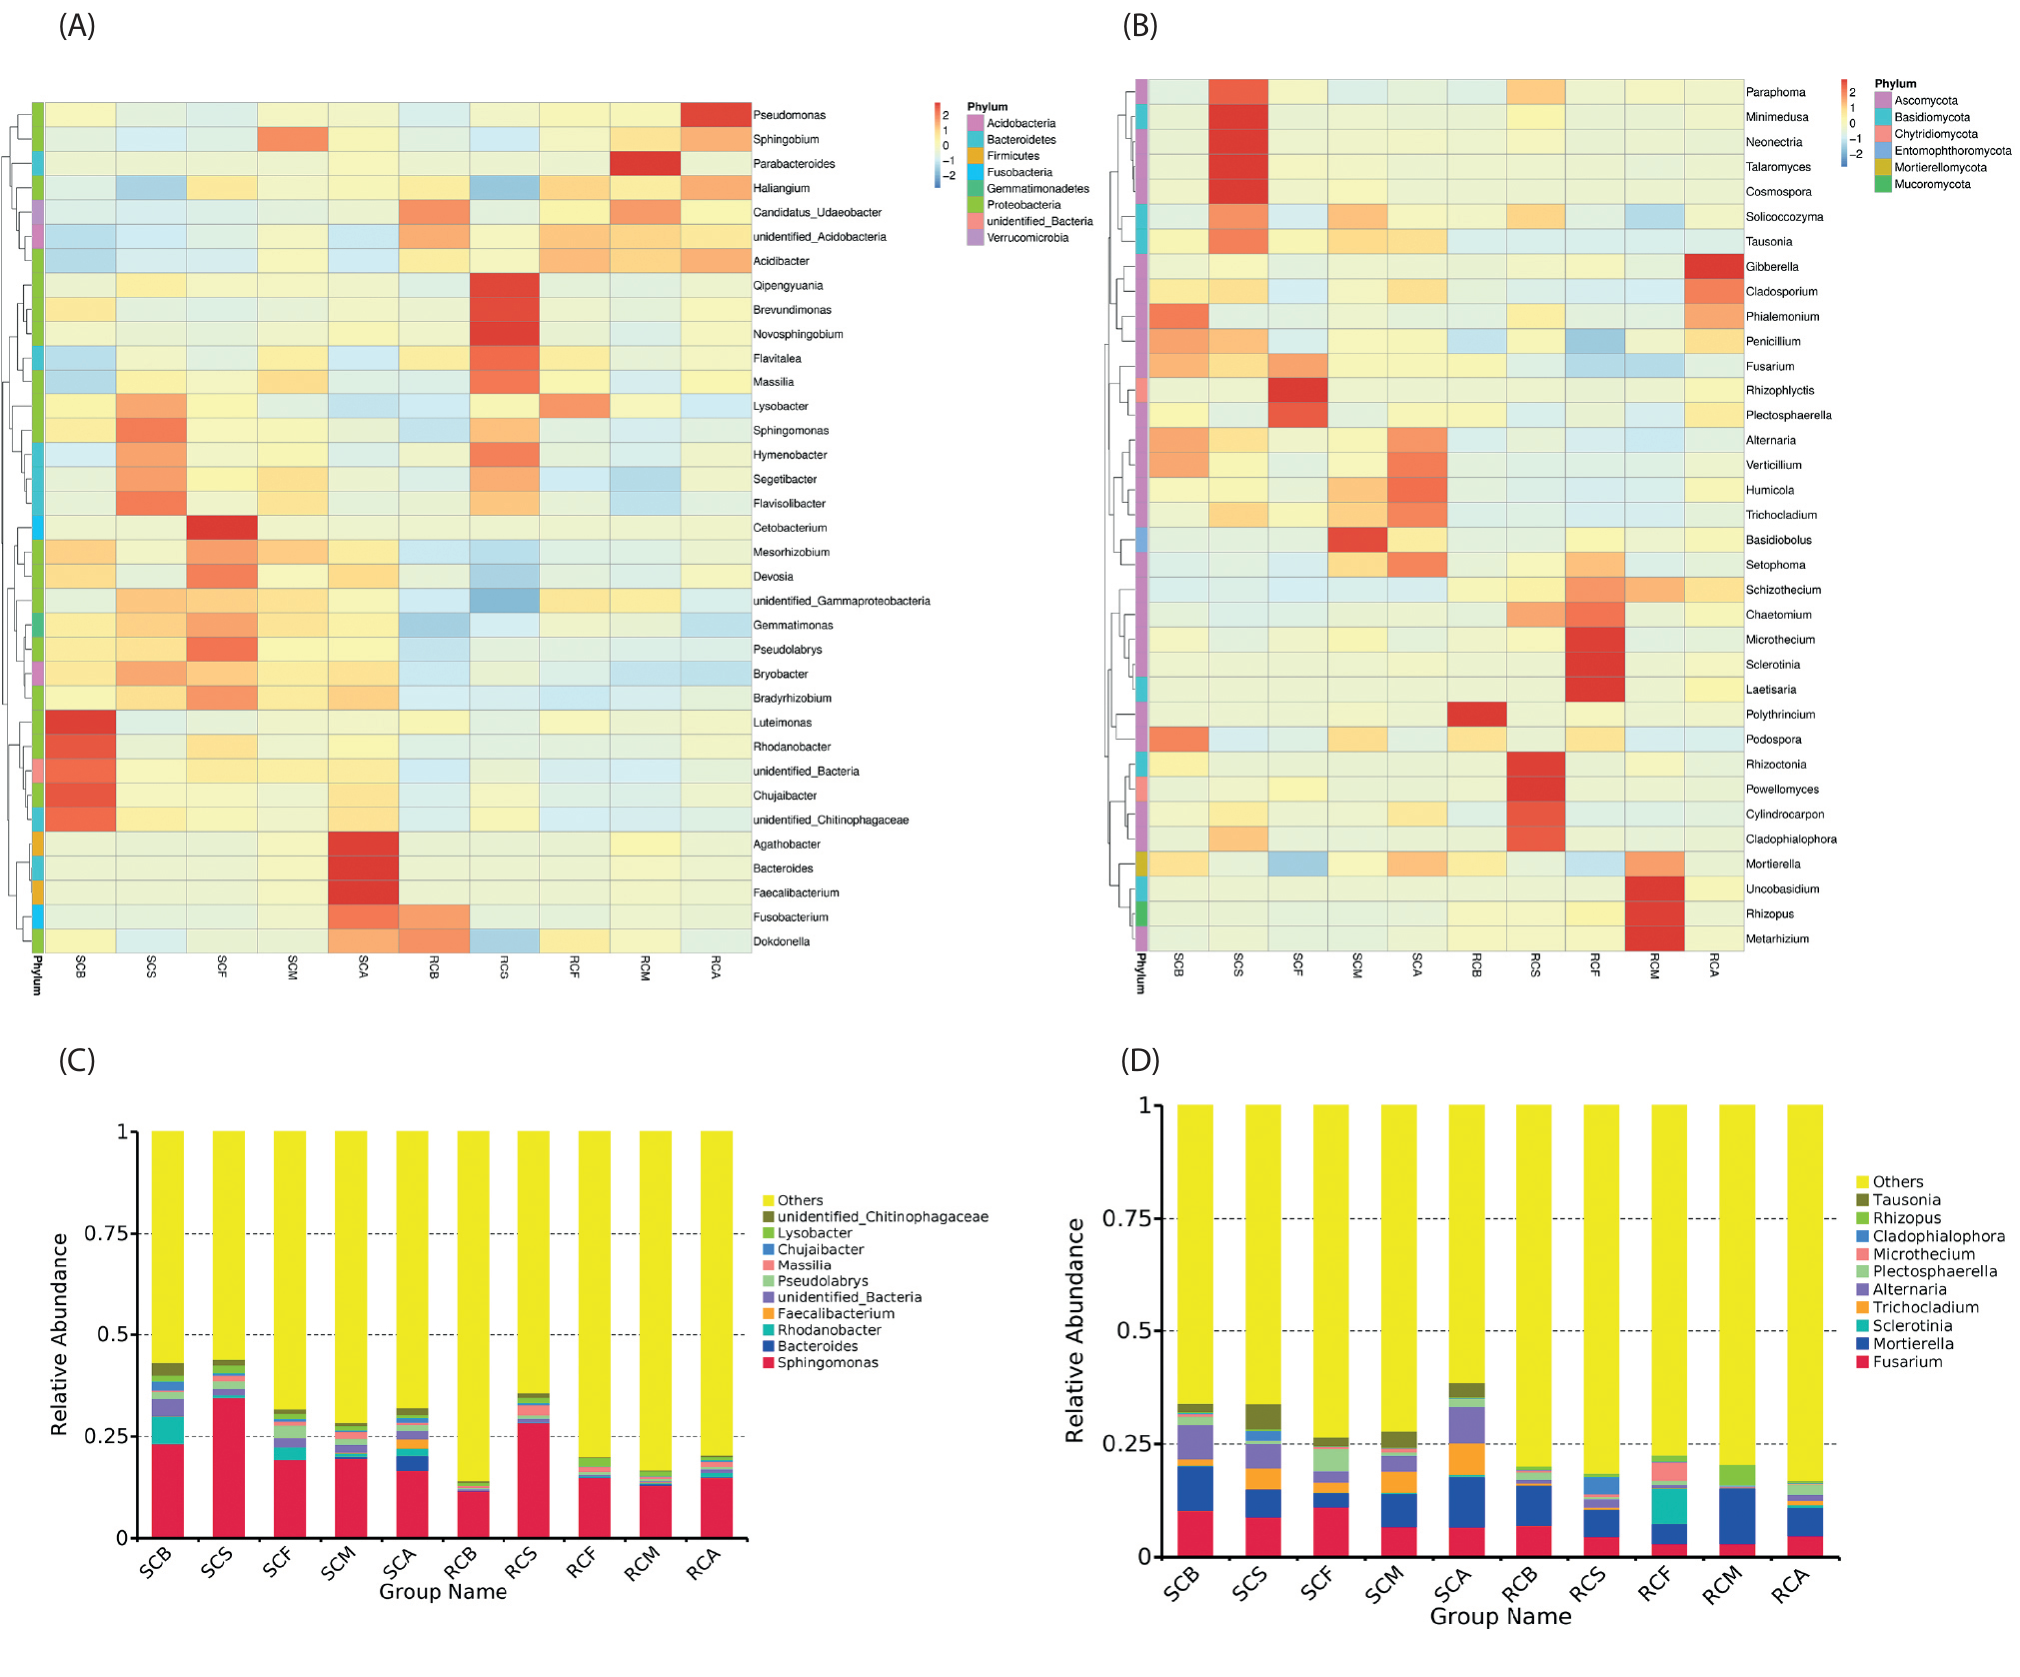
To further elucidate the effects of the two cropping patterns on soil microbial community structure at the genus level, the composition of bacteria and fungi was analyzed using heat maps and relative abundance maps (Fig. 5). The relative abundance of the top 35 genera of bacteria and fungi was analyzed by heat map, indicating significant differences in the community composition of bacteria and fungi genera between the SC and RC groups (Figs. 5A and B). The top 10 bacterial genera were Sphingomonas, Bacteroides, Rhodanobacter, Faecalibacterium, unidentified_Bacteria, Pseudolabrys, Massilia, Chujaibacter, Lysobacter, and unidentified_Chitinophagaceae (Fig. 5C). The relative abundance of Sphingomonas was highest in all periods (11.69–34.60%), and its abundance in the seedling period was the highest at 34.60% and 28.41% in the SC and RC groups, respectively. Compared with the SC group, the relative abundance of Lysobacter in the RC group during the flowering and after-harvest periods significantly (P = 0.011, P = 0.024) increased by 54.20% and 30.11%, respectively.
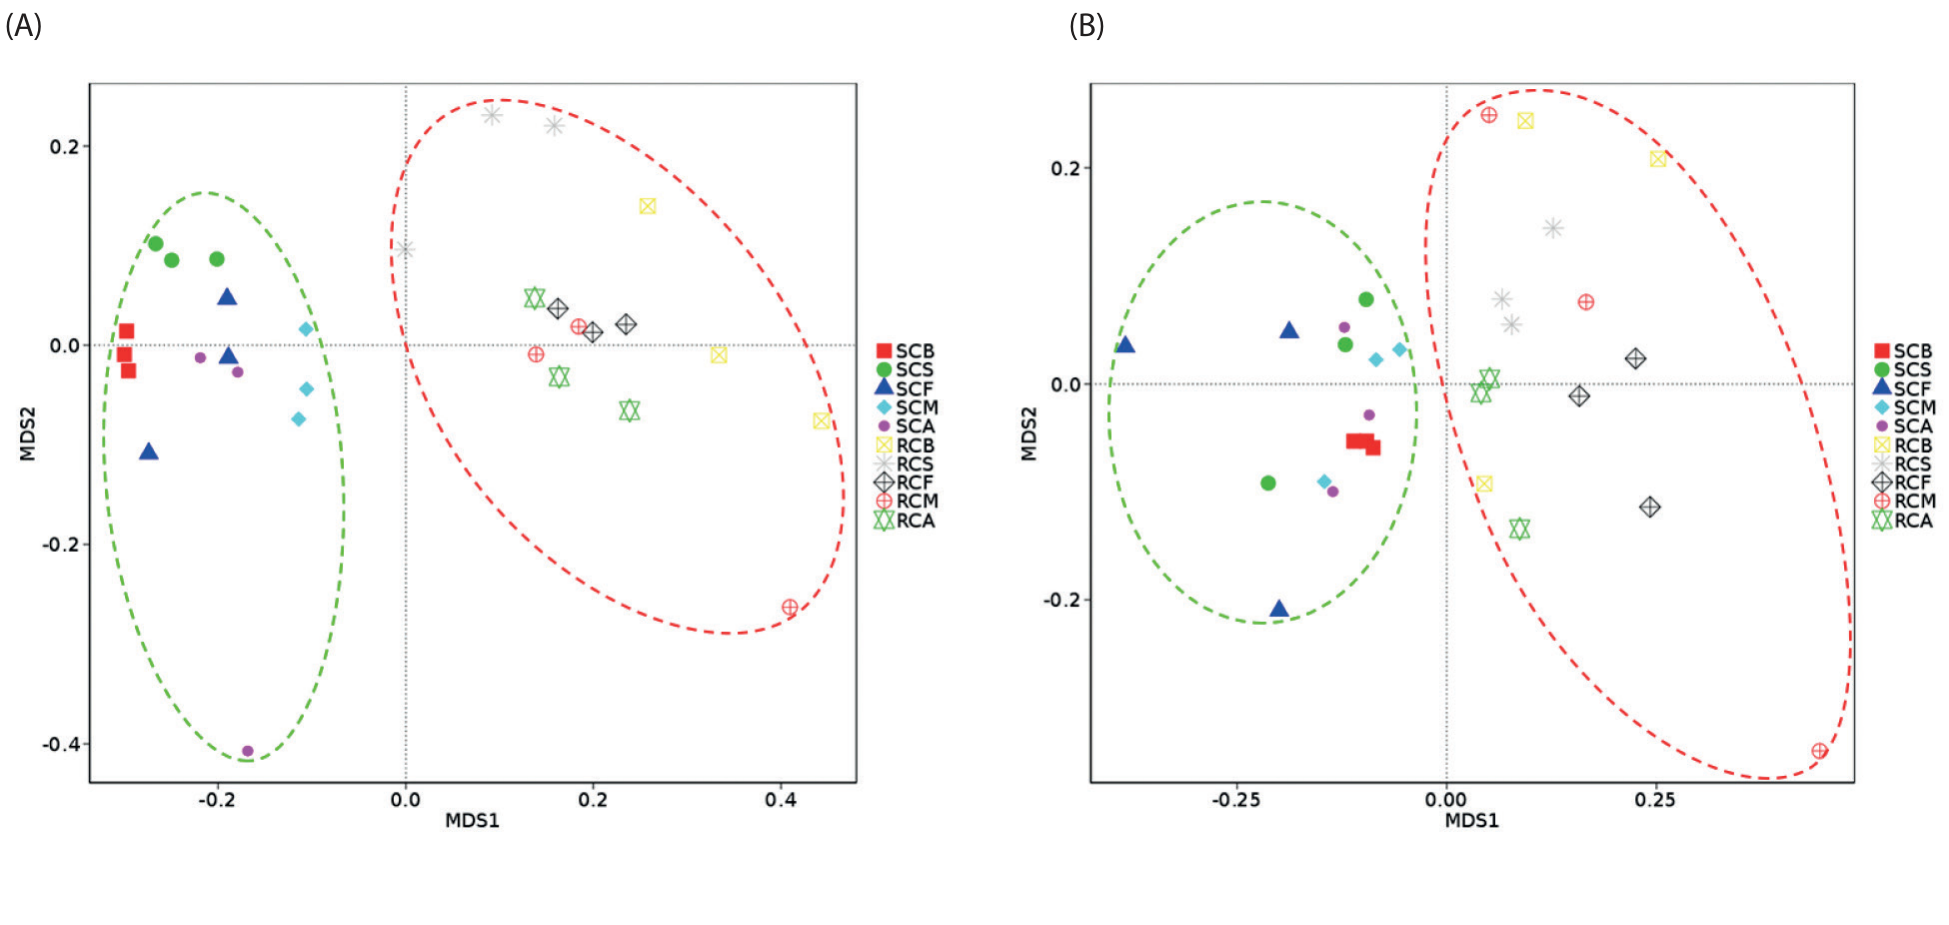
Fig. 6.
Analysis of microbial community structure. (A) Bacteria; (B) Fungi. SCB, SCS, SCF, SCM, and SCA represent before sowing, seedling, flowering, maturity, and after-harvest periods of continuous potato cropping, respectively. RCB, RCS, RCF, RCM, and RCA represent before sowing, seedling, flowering, maturity, and after-harvest periods of the rye-potato crop rotation, respectively.
For fungi, Fusarium, Mortierella, Sclerotinia, Tricho-cladium, Alternaria, Plectosphaerella, Microthecium, Cladophialophora, Rhizopus, and Tausonia were the top 10 genera (Fig. 5D). Compared with the SC group, the relative abundance of the pathogenic fungi Fusarium in the RC group significantly (P = 0.007, P = 0.014, P = 0.002, P = 0.049, P = 0.046) decreased in before sowing, seedling, flowering, maturity and after-harvest periods. Compared with the SC group, the relative abundance of the pathogenic fungus Alternaria in the RC group significantly (P = 0.0006, P = 0.004, P = 0.040, P = 0.010, P = 0.003) decreased in sowing, seedling, flowering, maturity, and after-harvest periods. The relative abundance of Fusarium decreased by 72.90% during the flowering period and was higher in all periods. The relative abundance of Alternaria in the RC group decreased by 66.48–93.44% throughout the potato planting period. Compared with the SC group, the relative abundance of Mortierella in the RC group significantly increased (P = 0.011, P = 0.003) by 37.90% and 65.36% during the flowering and maturity periods, respectively.
Microbial Community Structure
To visualize the similarity and dissimilarity in bacterial communities among soil samples, NMDS was performed based on bacterial OTUs of the 16S rRNA gene amplicon and fungal OTUs of the ITS rRNA gene amplicon sequencing using the Bray-Curtis metric (ANOSIM, bacteria: r = 0.8519, p = 0.01; fungi: r = 0.5657, p = 0.01). The bacterial samples from the SC and RC groups were distinct, with obvious differences in community structure (Fig. 6a). The fungal community was similar to that of bacteria (Fig. 6b), whereas the community structure was significantly different. These results showed that, compared with continuous potato cropping, rye-potato crop rotation changes the community structure of soil bacteria and fungi.
Discussion
Soil pH is one of the most important characteristics of soil. It plays a key role in the growth of plants and ani-mals. Continuous cropping of potatoes leads to soil acidi-fication. Studies have shown that long-term continuous cropping of various plants significantly reduces soil pH [33]. This study found that, compared with continuous cropping, rye-potato crop rotation significantly improved soil pH (Table 1). Several pathogenic fungi, including Fusarium and Pythium, adapt to slightly lower soil pH [34], while high pH inhibits Fusarium wilt [35]. Rye-potato crop rotation significantly improved soil OM and AN (Table 1). Soil OM content is an important condition for evaluating soil fertility levels and plays a crucial role in crop growth and development. Soil nitrogen can promote the decomposition of OM by soil microorganisms, and the high content of soil OM and nitrogen can help increase the diversity of the soil bacterial community [36, 37].
Rye-potato rotation significantly increased soil alkaline phosphatase activity, which was 1.23-fold higher than that of potato continuous cropping at the seedling stage. The activity of soil sucrase also increased significantly, which was 3.58-fold higher than that of continuous cropping fields at the flowering stage (Fig. 2). This is similar to previous findings that watermelon-wheat [38] and potato-legume [39] crop rotations improve soil enzyme activities. The level of soil enzyme activity is an important indicator of soil health. The soil enzyme system is the most active part of the soil that can activate soil OM and transform it into inorganic matter that can be absorbed by plants. It plays an important role in soil nutrient cycling and plant nutrient transformation and is considered a major feature that contributes to overall soil quality and microbial activity [40].
Compared with continuous cropping, rye-potato crop rotation significantly increased the diversity of bacteria and fungi (Tables 2 and 3). Soil microbial diversity is a key factor affecting soil health and quality, and agricultural treatment influences soil microbial diversity [41, 42]. This is consistent with previous findings that tomato-rice [43] and corn-American ginseng [44] crop rotations increase bacterial diversity, but this is in contrast to the result that a wheat-canola crop rotation reduces fungal diversity. Soil microbial communities play a central role in promoting the decomposition of OM and nutrient cycling, especially the abundant bacterial communities, which are indispen-sable to soil ecology [45]. Changes in the diversity of soil microbial communities are largely affected by soil environmental factors [46]. Soil microorganisms are important in inhibiting soil-borne diseases and inducing plant resistance [47]. Understanding the species and distribution of soil microorganisms is essential for controlling plant diseases.
This study showed that rye-potato crop rotation could improve the abundance of Actinobacteria and Acidobacteria in all periods, and the relative abundance of Firmicutes significantly increased in the maturity period (Fig. 4A). Similar results were observed with maize-peanut intercropping [48]. The relative abundance of Chloroflexi increased during the maturity and after-harvest periods. Acidobacteria and Chloroflexi can decompose carbon and participate in the organic carbon cycle [49]. Accord-ingly, the high abundance of Acidobacteria and Chloroflexi caused by rye-potato crop rotation may be due to higher soil OM content. The abundance of Actinobacteria is one of the key factors in the generation of bacteriostatic effects in soil [50, 51]. It is a bacteria that can inhibit soil diseases, including potato common scab [52], tobacco bacterial wilt [53], and banana Fusarium wilt [54]. Basidiomycota and Ascomycota were the predominant fungi in the soil (Fig. 4B), which is similar to the results of previous studies [55, 56]. Ascomycota comprises several plant pathogens [57]. The abundance of Ascomycota with rye-potato crop rotation significantly decreased by 49.26% and 21.24% at the maturity and after-harvest periods, respectively, compared with continuous cropping. Lysobacter imparts an inhibitory effect on plant diseases [58]. Fusarium and Alternaria in soil can cause Fusarium wilt and the early blight of potatoes. Rye-potato crop rotation significantly reduced the abundance of Fusarium and Alternaria at each period, while the relative abundance of Mortierella significantly increased during the maturity and flowering periods (Fig. 5D). This is similar to the findings of other scholars. They found that watermelon-wheat rotation reduced the incidence of Fusarium wilt. In addition, Mortierella is enriched in disease-free soil [59], and some strains have been shown to produce antifungal and antibacterial metabolites [60].
Changes in soil microbial community structure are very important for continuous potato cropping obstacles. The analysis of soil microbial community structure shows (Fig. 6) that for the continuous cropping of potatoes, rye-potato crop rotation can significantly change the community structure of soil bacteria and fungi. This is consistent with the research results of previous scholars, namely that tomato-rice crop rotation significantly affects the community structure of bacteria and fungi [61]. This indicates that rye-potato rotation can improve the structure of soil microbial communities.
Conclusion
Rye-potato crop rotation increases soil pH, OM, and soil alkaline phosphatase and sucrase activity, increasing the diversity of bacteria and fungi. This elucidated the effects of continuous cropping and rotation on potato soil physical and chemical properties and microbial community structure, thereby providing a theoretical basis for resolving obstacles related to continuous potato cropping.