

Introduction
The exposure of plants to both biotic and abiotic stress factors can significantly impede their growth and decrease productivity. Nearly 30% of arable land globally is vulnerable to drought, leading to alterations in agricultural practices [1]. Many abiotic stressors have detrimental effects on soil fertility and plant health, with drought stress being one of the most serious. As climate change becomes more severe, crop production will be adversely affected. The management of abiotic and biotic stress can be environmentally friendly and efficient through the use of rhizobacteria that promote plant growth. These bacteria play a crucial role in the plant’s growth process, both directly and indirectly [2]. Drought stress limits plant growth by reducing the photosynthetic rate. The primary reasons for photosynthesis reduction may be stomatal factors (loss of guard cells turgidity or CO2 triggered stomatal closure), nonstomatal factors (reduced photosynthetic activity in mesophyll tissue), or a combination of both [3]. Historically, okra has served as a valuable food source in economically underdeveloped countries in Asia and Africa, offering high levels of protein, carbohydrates, minerals, vitamins, and antioxidants [4]. An essential step in enhancing okra production is to increase the plant’s stress tolerance by activating novel genes, proteins, and metabolites [5]. When faced with stress, plant growth, and yield are significantly impacted, posing a threat to food security. Consequently, it is crucial to develop alternative strategies that increase the production of micronutrient-rich vegetables, protein, fiber, and antioxidants to address food and nutritional security concerns [6].
There has been a recent surge of interest in soil microbes. Among the most abundant groups of soil microbes, fungi, and bacteria play essential roles in regulating plant physiological processes in the rhizosphere [7]. Lower soil moisture levels (10-14%) lead to an increase in root hair density and length, which was primarily influenced by genetics [8] and hormonal regulation [9]. Microbes significantly influence the hormonal state of the root, contributing to its enhanced absorption of nutrients and water. This, in turn, promotes increased plant growth. Additionally, these microbes secrete biochemicals that facilitate their colonization and the formation of symbiotic relationships with the plant [10]. Plant growth-promoting rhizobacteria (PGPRs) increase the production of indole acetic acid (IAA) and abscisic acid (ABA) under water stress [11]. Plants can absorb nutrients and water more efficiently when treated with PGPR, which alters root architecture. The capability of microbes to decrease reactive oxygen species (ROS) generation and enhance antioxidant capacity remains a crucial factor for plant survival under drought stress [12].
Microbes in the soil, predominantly fungi and bacteria, play a critical role in the rhizosphere and can exert significant impacts on plant growth and development. The effects of abiotic stress on agricultural production can be substantial, but rhizobacterial inoculants show promise for mitigating these effects, making agriculture eco-friendly and more sustainable [13, 14]. Plant stimulants, plant conditioners, and bio-pesticides are all applications of these rhizobacteria. They have successfully reduced fertilizer inputs while enhancing nutrient use efficiencies, seed yield, and photosynthetic efficiency of crops such as durum wheat under drought conditions [15, 16].
Regardless of whether the soil is well-watered or water-scarce, rhizosphere microbes enhance soil fertility, plant growth, and resource efficiency through their biological processes. Some bacteria can colonize rhizospheres in soil, known as plant growth-promoting bacteria (PGPB). These bacteria have a reputation for colonizing rhizospheres and thrive under conditions of extreme dryness [17, 18]. Additionally, PGPR synthesizes phytohormones that resist abiotic stresses and promote cell growth [19]. The growth and development of plants are influenced by auxins like Indole 3 acetic acid [20]. There was increased root growth and lateral and root hair formation in plants that were inoculated with IAA-producing bacteria after inoculation [21, 22]. These root growth and hair formation are both important for increased water and nutrient uptake. As an organic fertilizer, PGPR can be used only in limited circumstances due to the lack of knowledge about the relationships between plants and microbes under drought stress conditions, as well as the composition, assembly, and structure of Rhizosphere microbes [23, 24]. With the growing frequency of heatwaves and droughts and the limited availability of irrigation water, research into and implementation of stress-mitigating solutions, such as PGPR, are crucial. Considering the role of rhizobacteria in enhancing plant growth, especially under water stress conditions, it was hypothesized that specific Rhizobacterium strains could positively impact the growth and physiological characteristics of okra plants, thereby improving their drought tolerance. Additionally, bacterial consortia were expected to exhibit a synergistic effect, providing more effective regulation of okra physiology related to drought tolerance compared to individual bacterial strains. The research involved laboratory experiments with the following specific objectives: (i) assessing the drought tolerance potential of isolated bacterial strains, (ii) examining the effect of bacteria with differing drought tolerance abilities on the growth of okra seedlings subjected to water stress, and (iii) assessing whether bacterial consortia are effective in regulating okra physiology related to drought tolerance.
Material and Methods
The present study was conducted to examine PGPRs individually and in consortium to determine improvement in okra growth. For this purpose, 10 pre-isolated, characterized and identified strains S10 (Bacillus aryabhattai), ZM63 (Bacillus subtilis), ZM31 (Bacillus aryabhattai), ZM27 (Paenibacillus polymyxa), [25], AN35 (Bacillus megaterium), AN24 (Bacillus megaterium) [26], ZR3 (Bacillus subtilis), ZE11 (Paenibacillus sp.), ZE15 (Bacillus subtilis), ZE32 (Bacillus megaterium) [27] were collected Soil Microbiology and Biotechnology Laboratory’s culture bank. The accession numbers of the studied strains were KX788862, KX788861, KX788860, KX788859, MN005929, MN005926, MN007185, MN003399, MN003400, MN003401, respectively.
Identifying the MIC of Bacteria Strains Under PEG-6000
The MIC of drought-tolerant rhizobacterial strains was determined by inoculating the 48-hour-old culture on an agar plate. The agar plates consisting of Luria-Bertani (LB) medium were amended with PEG- 6000. The concentration of PEG-6000 in the growth media was increased from an initial 2% until it hindered the growth of bacteria. PEG-6000 was used to measure the lowest concentration at which visible bacterial colony growth was stopped. The experiment was repeated three times. The plates were incubated in an incubator at 28±1ºC for 72 hours to determine the MIC of drought-tolerant bacteria [28].
Drought Tolerance Assay
The chosen rhizobacterial strains were evaluated for their growth patterns under varying levels of PEG- 6000 (0, 2, 4, 6, and 8%) having osmotic potential values (-0.14, -0.36, -0.66, -1.03 MPa, respectively) in a general-purpose broth culture. For this purpose, general-purpose broth modified with PEG-6000 was papered and autoclaved. A loop full of 24 hour old bacterial colonies was dipped in sterilized broth, and the flask was sealed with Parafilm at 30±1ºC and incubated in a rotary shaking incubator. Each flask was used in triplicate to remove/reduce errors. The optical density was determined at 600 nm after 24, 48, 72, and 96 hours using an Ultra-Violet (UV)- visible spectrophotometer. The most effective strains were preserved in 50% (v/v) glycerol solution at -20ºC for further investigation [29, 30].
Indole Acetic Acid Production by PGPR Strains Under Drought Stress
Testing was conducted on bacteria exhibiting maximum growth on PEG-amended broth media with and without L-tryptophan (L-tryp) supplementation as Bric’s method [31]. Incubation of an overnight-grown bacterial culture in LB liquid media amended with 5% L-tryp and 4% PEG was performed in a rotary shaking incubator (100 rpm) at 32ºC for 72 hours. Color development was recorded by centrifuging the tubes at 4500g for 20 minutes and mixing the supernatant with Salkowski reagent (0.5 M FeCl3.6H2O and 35% H2SO4). Using a UV-visible spectrophotometer, the samples and IAA standards (0 to 100 mg kg-1) were measured at 535 nm to determine their absorbances (Carry 60; Agilent, USA). The IAA concentration was calculated from known conc. standards curve. A parallel set without L-tryp was also prepared to compare the results. The entire experiment was repeated three times. The four most efficient strains, ZE15 (Bacillus subtilis), ZE11 (Paenibacillus sp.), ZE32 (Bacillus megaterium), and ZR3 (Bacillus subtilis), were selected for further testing based on EPS production and IAA production ability [31].
Studying PEG-Induced Droughts and IAA Production in Selected Strains
Selected strains were tested for growth and IAA production under PEG-induced drought stress. Various levels of drought were applied to the selected strains, namely 0, 2, 4, 6, and 8% of PEG-6000. There were three repetitions of the experiment. Incubation was carried out in a rotary shaking incubator at 100 rpm for 72 hours at 28ºC, using a 48-hour-old culture inoculated with broth culture tubes. A UV-Vis spectrophotometer measuring absorbance at 600 nm wavelength was used to monitor growth after 24, 48, and 72 hours. The production of IAA and EPS by the rhizobacterial strains under PEG-induced drought stress was determined with a UV-visible spectrophotometer as described in [32] and [33], respectively.
Compatibility Assay
An assessment of compatibility between the selected strains was conducted. Agar plates were crossed-streaked with colonies of the selected strains after 48 hours of incubation. The inhibition of growth at the point of intersection indicated that those strains are incompatible with each other and vice versa. The whole experiment was replicated thrice to minimize the error. The best compatible combinations were selected for further evaluation under controlled and natural conditions [34].
Soil Sample Collection and Examination
This soil was collected from the Department of Soil Science research area at the Islamia University of Bahawalpur and placed in polythene bags for further study. The soil was air-dried in the shade, ground, mixed, sieved with a 2mm stainless steel mesh, and analyzed for its physical and chemical properties using a standard protocol from [35]. (Table 1).
Screening of Okra for Drought Tolerance Based on EC50 (Effective Control to 50% Growth Inhibition)
Six hundred grams of soil were weighed and amended with PEG-6000 at 0, 2, 4, 6, and 8%. Jars were placed in a growth room at 70% relative humidity with light intensity of 1000 lux, 12 h/day at 28±2ºC, and 12 h dark at 15±2ºC. The experiment was repeated three times and the jars were using a completely randomized design (CRD). Seeds of okra were purchased from the local market of Bahawalpur.
Each jar was seeded with ten seeds. Immediately following germination, the density of plants was maintained at three plants per jar. The Hoagland solution of half strength was used for irrigation and nutrient requirements of the crop [36]. The seedlings were harvested 25 days after planting, and root growth was measured with a root scanner. The growth parameters were determined, including the length of the shoot and root and the fresh and dry biomass of both shoot and root. The level of drought stress at which seedlings showed 50% growth reduction was selected for further evaluation.
Jar Trial for Screening the Effective Drought-Tolerant Sole and Consortium Rhizobacterial Strains for Improving the Okra Growth Under Controlled Conditions
The drought-tolerant properties of the selected isolates were evaluated in jars under controlled conditions by performing a controlled experiment. The most compatible drought-tolerant strains were processed under axenic conditions after compatibility testing. Drought-tolerant rhizobacterial strains with the maximum optical density were used in a three-replication jar experiment. Seeds were treated by dipping them in the bacterial broth for 15 minutes before sowing in sterilized jars filled with soil and 4% PEG-6000 (-0.36 MPa). The jars were supplied with nutrients using a half-strength Hoagland solution. The experiment was arranged using a completely randomized design with three replications. Eleven (11) treatments were established, including the application of single and combined inoculations of the selected compatible strains as T1: Control, T2: ZE15 (Bacillus subtilis), T3: ZE11(Paenibacillus sp.), T4: ZE32 (Bacillus megaterium), T5: ZR3(Bacillus subtilis), T6: ZE15 (Bacillus subtilis) +ZE11 (Paenibacillus sp.), T7: ZE15 (Bacillus subtilis) +ZE32 (Bacillus megaterium), T8: ZE15 (Bacillus subtilis) + ZR3 (Bacillussubtilis), T9: ZE11(Paenibacillus sp.), + ZE32 (Bacillus megaterium), T10: ZE11 (Paenibacillus sp.)+ZR3(Bacillus subtilis) and T11: ZE32 (Bacillus megaterium)+ZR3 (Bacillus subtilis). The same treatment set was also observed under drought conditions. Ten (10) seeds per pot were sown, and three plants were maintained in each pot throughout the growing process for the germination population to increase. After 20 days of sowing, data on various growth parameters were collected.
The root and shoot lengths were measured using a measuring tape, and the weight was recorded using an analytical balance. The samples were air-dried and then oven-dried at 65°C for three days. The dry weight was measured using the electrical balance. This study used a root scanner (Win RHIZO Pro, STD, 2017 Netherland) to measure the root volume, diameter, and surface area and a leaf scanner (Win FOLIA Pro, T221B, 2016, Netherlands) to measure the surface area of the leaves.
Statistical Analysis
The Analysis of variance (ANOVA) for experiments was constructed using Statistics 8.1® software using a CRD design in the factorial arrangement. Least Significant Difference (LSD) was used at a significance level of 5% at the end of the study when comparing means between treatments [37].
Results
The objective of the present investigation was to enhance okra’s ability to withstand drought by application of plant-growth-promoting rhizobacteria (PGPR) through the production of the phytohormone (IAA) and other growth-promoting traits. Laboratory bioassays were performed, followed by pot and field experiments to assess the impact of IAA-producing PGPR on okra growth, physiology, and yield under water-limited conditions. Four efficient IAA-producing strains, ZE15 (Bacillus subtilis), ZE11 (Paenibacillus sp.), ZE32 (Bacillus megaterium), and ZR3 (Bacillus subtilis), were selected from a group of ten pre-isolated and characterized rhizobacterial strains based on their IAA production ability. Several strains of these plants were then tested under polyethylene glycol (PEG-6000) induced drought stress conditions for their drought tolerance and IAA production.
Table 2.
Growth in terms of optical density (OD600) of rhizobacterial isolates.
Screening of Drought-Tolerant Rhizobacteria Based on Growth
The drought tolerance of the strains was confirmed by growing them in a liquid culture containing 4% PEG-6000, and their growth was determined using a UV-visible spectrophotometer (Model: Cary60; Agilent, USA). The results showed that all the isolates grew in the PEG-6000 amended medium. However, the strains ZE15 (Bacillus subtilis), ZE11 (Paenibacillus sp.), ZE32 (Bacillus megaterium), and ZR3 (Bacillus subtilis) showed better growth compared to the other isolates (Table 2).
Measurement of IAA Production by the Rhizobacterial Strains
IAA production in the presence and absence of L-Tryptophan was evaluated in the selected strains that grew in the presence of PEG (Table 3). There was a variation in the IAA production between all the strains tested. The isolate ZE15 (Bacillus subtilis) showed the highest IAA production (10.23 µM) ability, followed by ZE32 (Bacillus megaterium) 9.07 µM, ZE11 (Paenibacillus sp.), and ZR3 (Bacillus subtilis). The isolate S10 did not produce any IAA in both conditions. The four strains with the greatest IAA production ability (ZE15, ZE11, ZE32, and ZR3) were chosen for further experimentation. The results were confirmed through three replications of the bioassays.
Determination of Minimum Inhibitory Concentration (MIC) of PEG-6000 for Rhizobacterial Isolates
The selected rhizobacterial isolates ZE15 (Bacillus subtilis), ZE11 (Paenibacillus sp.), ZE32 (Bacillus megaterium), and ZR3 (Bacillus subtilis) were tested for their ability to grow under PEG-induced water-stressed conditions, and MIC was recorded. The results revealed that the isolates ZE15 (Bacillus subtilis) and ZE11 (Paenibacillus sp.) performed better under drought-stressed conditions and showed growth at a higher level of PEG-6000 in agar plate assay. The isolates ZE32 (Bacillus megaterium) and ZR3 (Bacillus subtilis) showed an increase of up to 10 and 12% concentration of PEG-6000, respectively. However, the isolates ZE15 (Bacillus subtilis) and ZE11 (Paenibacillus sp.) were more efficient in growing under drought-stressed conditions. These isolates showed growth up to 18% concentration of PEG-6000.
Table 3.
Indole-3-acetic acid (IAA) production by rhizobacterial strains with and without L-Tryptophan.
The Impact of Drought Stress Caused by PEG on Growth and IAA Production Capability in Selected Strains
The effects of varying levels of PEG-induced drought stress on the growth and production of IAA by rhizobacterial strains were examined. The bacterial strains were drought-tolerant and produced IAA. The strains were monitored for development and IAA production every 24 to 72 hours. The results in Table 3 showed that higher levels of PEG significantly reduced the growth of the rhizobacterial strains and caused an earlier transition to the stationary phase. The isolates displayed varying responses to drought stress, with the ZE11 (Paenibacillus sp.) isolate demonstrating the best growth at 8% PEG concentration. Because of the different stress levels, the strains also varied in their ability to produce IAA under normal and stressed conditions. After 72 hours under normal conditions, the highest concentration of IAA (55 g/mL) was recorded in ZE11 (Paenibacillus sp.), while the lowest concentration of IAA was recorded in ZR3 (Bacillus subtilis) at 8% PEG concentration after 72 hours. A rapid increase in IAA production was recorded by the tested isolates up to 48 hours, while after that, the production of IAA was non-significant at 8% of the concentration of PEG. The findings showed that the IAA production capabilities of the isolates varied significantly. (Table 4).
The Growth-Enhancing Properties of the Selected Rhizobacterial Strains for Plants
Further evaluation of the selected isolates for various plant growth-promoting attributes was conducted. A preselected and identified set of rhizobacteria (Paenibacillus sp. strain ZE11 [MN003399], Bacillus subtilis strain ZE15 [MN003400], Bacillus megaterium strain ZE32 [MN003401]) and rhizobacterial strains (Bacillus subtilis strain ZR3 [MN007185]) was tested individually and in combination. The strains had previously been characterized and shown to produce high levels of exopolysaccharides (EPS), siderophore production, urease activity, hydrogen cyanide production, and catalase activity, along with the ability to oxidize substances. Previously, in a growth room trial, research has shown that their root colonization and compatibility were both successful (Iqbal et al., 2020).
Screening of Okra for Drought Tolerance Based on EC50 (Effective Control to 50% Growth Inhibition)
Okra seedlings were evaluated for their drought tolerance at varying levels of PEG in controlled conditions and assessed for growth characteristics. The treatments were T1 = Control, T2 = 2% PEG, T3 = 4% PEG, T4 = 6% PEG, and T5 = 8% PEG. The seedlings showed variable results under 0, 2, 4, 6, and 8% levels of PEG-6000. In response to a 2% drought stress level, Okra seeds showed improved germination rates, dry seedling weights, shoot lengths, and root lengths compared to control seeds. All the growth parameters showed a 50% growth reduction at level 4%. At a drought level of 6 and 8%, the performance of all the growth parameters declined. The level (4%) where okra showed a 50% growth reduction was selected for further experimentation (Table 5).
Table 4.
Impact of various concentrations of PEG-6000 on the growth and production of IAA by rhizobacterial strains.
Potential of Drought Tolerant IAA Producing Rhizobacteria to Improve the Fresh and Dry Weight of Okra in Jar Trial
The evaluated strains were tested for their ability to promote growth in okra plants under both control and drought conditions. Inoculation of seeds with drought-tolerant and IAA-producing rhizobacteria significantly improved okra growth in control conditions (Table 6). The statistical analysis indicated that Treatment T6, consisting of Bacillus subtilis (ZE15) and Paenibacillus sp. (ZE11), led the highest values for growth parameters such as fresh shoot weight, root fresh weight, shoot dry weight, and root dry weight, with increases of 25, 30, 24, and 26% respectively, compared to the uninoculated control. The same treatment (T6) resulted in the maximum growth parameters, with increases of 18, 23, 22, and 25%, respectively, compared to the uninoculated control under water stress.
Potential of Drought Tolerant IAA Producing Rhizobacteria to Improve Growth Parameters of Okra in Jar Trial
A further evaluation was conducted on the selected strains to determine whether they could promote growth in okra under controlled and drought conditions. A seed inoculum containing drought-tolerant and IAA-producing rhizobacteria significantly enhanced the growth of okra under control conditions (Table 7). Based on statistical analysis, Treatment T6 ZE15 (Bacillus subtilis) + ZE11 (Paenibacillus sp.) showed maximum growth parameters such as root length, shoot length, No. of Seed germinated, and plant height, resulting in 25, 25, 24, and 26% increases in root length, shoot length, No. of Seed germinated, and plant height, respectively, over the control group that was not inoculated. The same treatment (T6) exhibited the maximum results for the growth parameters with 22, 22, 23, and 22% increases over the uninoculated control under the water-stressed conditions.
Potential of Drought Tolerant and IAA-Producing Rhizobacteria to Improve Root Diameter of Okra in Jar Trial
Fig. 1 presents the effectiveness of different rhizobacterial strains on control and drought treatments in okra plants. The results showed a 23% decrease in plant height in water-stressed seedlings compared to well-watered seedlings. When the bacterial strains were applied solely or in combination, the reduction in root diameter was significantly more significant than when drought treatment was applied. The combination of the bacterial strains, however, showed better results than the application of just one strain alone in terms of results. Among sole inoculation, a maximum 12% increase by strain ZE15 (Bacillus subtilis) (T2) followed by a 10% increase by strain ZE11(Paenibacillus sp) (T3) than uninoculated control under average conditions. However, the co-inoculation of ZE11 and ZE15 (T6) showed the most significant increase of 27% compared to the uninoculated control under normal conditions. Co-inoculation by ZE15 (Bacillus subtilis) + ZE32 (Bacillus megaterium (T7) was a subsequent treatment with a 20% increase in plant height. However, in stressed conditions, the maximum results (24%) were recorded in treatment (T6), where consortium ZE15 (Bacillus subtilis) + ZE11 (Paenibacillus sp) was applied as compared to uninoculated control followed by treatment T7 (20%) where ZE15 (Bacillus subtilis) + ZE11 (Paenibacillus sp.) was used.
Table 5.
Screening of okra for drought tolerance based on EC50 (effective control to 50% growth inhibition).
[i] *Where SFW = Shoot Fresh Weight, RFW = Root Fresh Weight, SDW = Shoot Dry Weight, RDW = Root Dry Weight, RL = Root Length, SL = Shoot Length, LSA = Leaf Surface Area, RV = Root Volume, RSA = Root Surface Area and PH = Plant Height. T1 = Control, T2 = 2% PEG, T3 = 4% PEG, T4 = 6% PEG, and T5 = 8 % PEG
Table 6.
Potential of drought tolerant IAA producing rhizobacteria to improve the fresh and dry weight of okra plant in jar trial.
Table 7.
Potential of drought tolerant IAA producing rhizobacteria to improve growth parameters of okra in jar trial.
Investigating the Potential of Drought-Tolerant IAA-Producing Rhizobacteria to Increase the Root Surface Area of Okra in a Jar Trial
This graph displayed the effectiveness of bacterial strains in soil along with combined application to improve the root surface area of okra plants under normal and drought conditions (Fig. 2). Our results showed a 23% decrease in surface area in drought-stressed seedlings compared to well-watered seedlings. The bacterial strains applied in different treatments significantly improve root diameter compared with drought treatment. A combination of inoculating different types of bacteria inoculated simultaneously achieved better results than inoculating one strain at a time. Among the sole inoculations, (ZE15) T2 (Bacillus subtilis) showed the most significant increase of 17%, followed by T3 (Paenibacillus sp.) (ZE11) with an increase of 12%, compared to the uninoculated control under drought conditions. Under drought conditions, Paenibacillus sp. (ZE11) and Bacillus subtilis (ZE15) (T6) co-inoculation showed the highest difference in increase of 23% as compared to the control where no bacteria were inoculated. The subsequent treatment (T7) was inoculated with ZE15 (Bacillus subtilis) +ZE32 (Bacillus megaterium), which showed better results where a 20% increase was recorded.
IAA-Producing Rhizobacteria with Drought Tolerance to Improve Root Volume of Okra Grown in Jars
The sole and co-inoculation effectiveness of bacterial strains on root volume in control and drought conditions are indicated in Fig. 3. Our results showed a significant decrease of 23% in root volume in drought seedlings than well-watered seedlings. The bacterial strains applied in different treatments significantly improve root volume compared with drought treatment. However, combined inoculation of bacterial strains showed better results than sole inoculation. When ZE11 (Paenibacillus sp.) + ZE15 (Bacillus subtilis) were inoculated together, there was a maximum increase of 24% compared with an un-inoculated control under control conditions. Under stressed conditions, the same treatment (T6) exhibits the maximum results (22%) compared to the uninoculated control. The following treatment (T7), inoculated with ZE15 (Bacillus subtilis) +ZE32 (Bacillus megaterium), showed better results where an 11 and 13% increase was recorded in both control and stress conditions, respectively.
Examining the Potential of Drought-Tolerant IAA-Producing Rhizobacteria to Enhance the Leaf Area of Okra in a Jar Trial
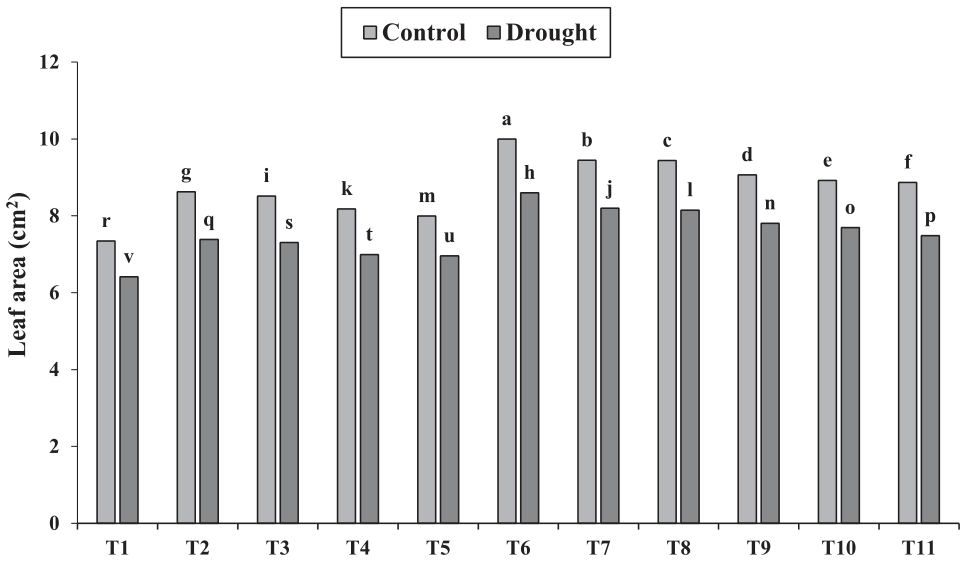
The graph showed the result of inoculated bacterial strains in sole or combined application on leaf area in control and drought conditions, as shown in Fig. 4. All inoculated bacterial strains showed significant enhancement in leaf area compared to the un-inoculated control treatment. Among sole inoculation, a maximum 14 and 13% increase by strain ZE15 (Bacillus subtilis) (T2) followed by a 12% increase by strain ZE11 (Paenibacillus sp.) (T3) than un-inoculated control under normal and stressed conditions. The combined application of both bacterial strains did, however, produce more significant results than the sole application of the strains. The treatment T6 ZE11 (Paenibacillus sp.) + ZE15 (Bacillus subtilis) showed maximum improvement with 27 and 25% increases, followed by T7 ZE15 (Bacillus subtilis) + ZE32 (Bacillus megaterium) with 22 and 21% increase on leaf area under both conditions.
Fig. 1.
Potential of drought tolerant IAA producing rhizobacteria to improve root diameter of okra in a jar trial. T1: Control, T2: ZE15 (Bacillus subtilis), T3: ZE11(Paenibacillus sp.), T4: ZE32 (Bacillus megaterium), T5: ZR3(Bacillus subtilis), T6: ZE15 (Bacillus subtilis) +ZE11 (Paenibacillus sp.), T7: ZE15 (Bacillus subtilis) +ZE32 (Bacillus megaterium), T8: ZE15 (Bacillus subtilis) + ZR3 (Bacillussubtilis), T9: ZE11(Paenibacillus sp.), + ZE32 (Bacillus megaterium), T10: ZE11 (Paenibacillus sp.)+ZR3(Bacillus subtilis) and T11: ZE32 (Bacillus megaterium)+ZR3 (Bacillus subtilis). Means with different letters are significantly different at p≤0.05.
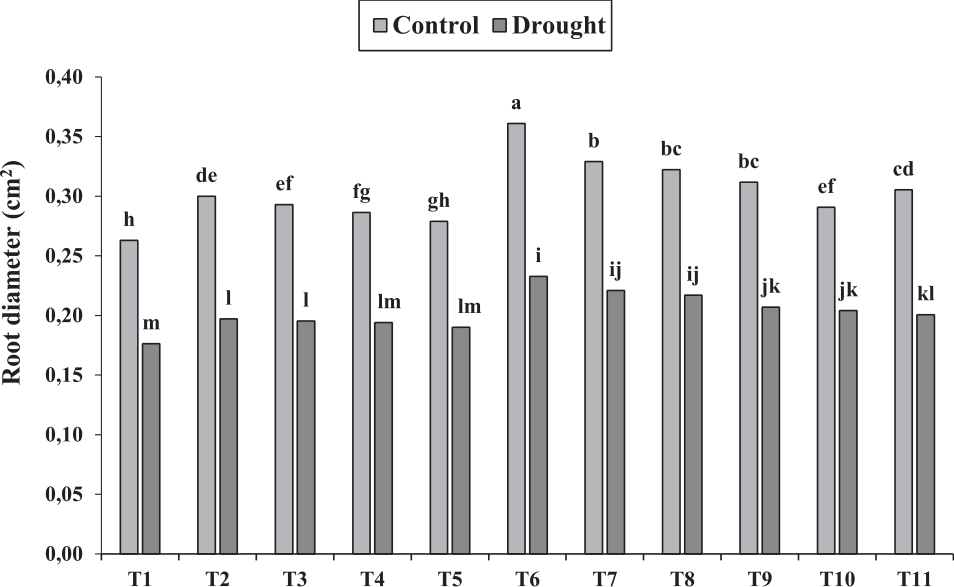
Fig. 2.
Potential of drought tolerant IAA producing rhizobacteria to improve root surface area of okra under a jar trial T1: Control, T2: ZE15 (Bacillus subtilis), T3: ZE11(Paenibacillus sp.), T4: ZE32 (Bacillus megaterium), T5: ZR3(Bacillus subtilis), T6: ZE15 (Bacillus subtilis) +ZE11 (Paenibacillus sp.), T7: ZE15 (Bacillus subtilis) +ZE32 (Bacillus megaterium), T8: ZE15 (Bacillus subtilis) + ZR3 (Bacillussubtilis), T9: ZE11(Paenibacillus sp.), + ZE32 (Bacillus megaterium), T10: ZE11 (Paenibacillus sp.)+ZR3(Bacillus subtilis) and T11: ZE32 (Bacillus megaterium)+ZR3 (Bacillus subtilis). Means with different letters are significantly different at p≤0.05.
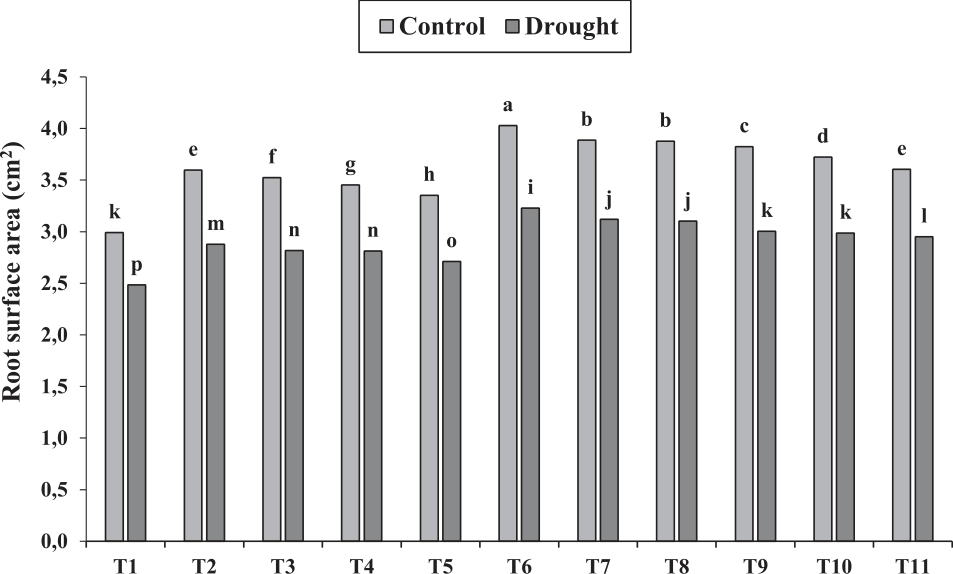
Fig. 3.
Potential of drought tolerant and IAA-producing rhizobacteria to improve root volume of okra in jar trial T1: Control, T2: ZE15 (Bacillus subtilis), T3: ZE11(Paenibacillus sp.), T4: ZE32 (Bacillus megaterium), T5: ZR3(Bacillus subtilis), T6: ZE15 (Bacillus subtilis) +ZE11 (Paenibacillus sp.), T7: ZE15 (Bacillus subtilis) +ZE32 (Bacillus megaterium), T8: ZE15 (Bacillus subtilis) + ZR3 (Bacillussubtilis), T9: ZE11(Paenibacillus sp.), + ZE32 (Bacillus megaterium), T10: ZE11 (Paenibacillus sp.)+ZR3(Bacillus subtilis) and T11: ZE32 (Bacillus megaterium)+ZR3 (Bacillus subtilis). Means with different letters are significantly different at p≤0.05.
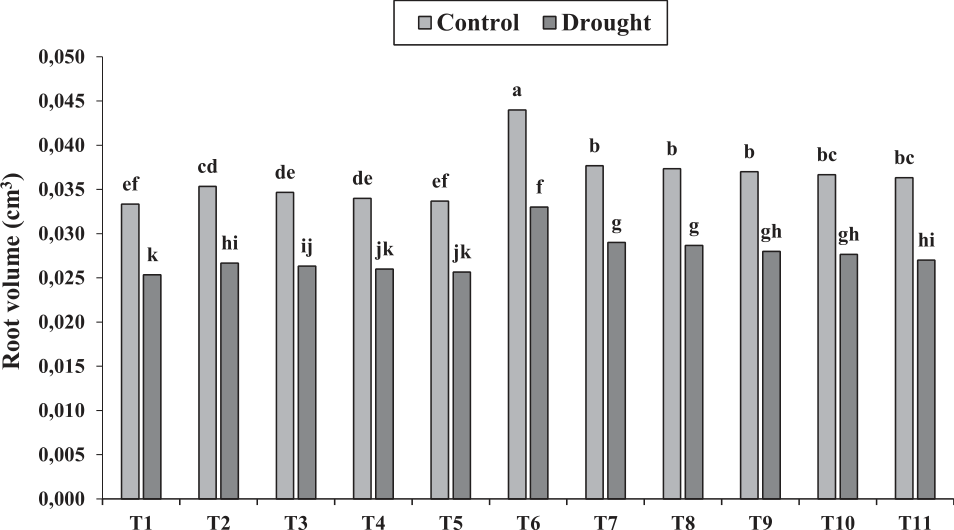
Fig. 4.
Potential of drought tolerant and IAA-producing rhizobacteria to improve leaf area of okra in a jar trial T1: Control, T2: ZE15 (Bacillus subtilis), T3: ZE11(Paenibacillus sp.), T4: ZE32 (Bacillus megaterium), T5: ZR3(Bacillus subtilis), T6: ZE15 (Bacillus subtilis) +ZE11 (Paenibacillus sp.), T7: ZE15 (Bacillus subtilis) +ZE32 (Bacillus megaterium), T8: ZE15 (Bacillus subtilis) + ZR3 (Bacillussubtilis), T9: ZE11(Paenibacillus sp.), + ZE32 (Bacillus megaterium), T10: ZE11 (Paenibacillus sp.)+ZR3(Bacillus subtilis) and T11: ZE32 (Bacillus megaterium)+ZR3 (Bacillus subtilis). Means with different letters are significantly different at p≤0.05.
Potential of Drought Tolerant IAA Producing Rhizobacteria to Improve Soil Plant Analysis Development (SPAD) Value of Okra in Jar Trial
The results of the chlorophyll content, shown in Fig. 5, indicated that bacterial inoculation led to a significant improvement in both control and drought conditions compared to the uninoculated control treatment. The sole and combined application of bacterial strains improved chlorophyll content compared to the drought treatment. As a result, it was found that the combined application of the two bacteria strains showed better results than the sole application of a single strain. Among the sole inoculations, Bacillus subtilis (ZE15) (T2) showed the highest increase of 13%, followed by Paenibacillus sp. (ZE11) (T3) with a rise of 11% compared to the uninoculated control under drought conditions. Compared to the uninoculated control under drought conditions, a co-inoculation of Paenibacillus sp. (ZE11) and Bacillus subtilis (ZE15) showed a 24% increase in SPAD value. In contrast, a combination of Bacillus subtilis (ZE15) and Bacillus megaterium (ZE32) (T7) produced a 22 percent increase in SPAD value.
Fig. 5.
Potential of drought tolerant and IAA-producing rhizobacteria to improve SPAD value of okra grown in jars T1: Control, T2: ZE15 (Bacillus subtilis), T3: ZE11(Paenibacillus sp.), T4: ZE32 (Bacillus megaterium), T5: ZR3(Bacillus subtilis), T6: ZE15 (Bacillus subtilis) +ZE11 (Paenibacillus sp.), T7: ZE15 (Bacillus subtilis) +ZE32 (Bacillus megaterium), T8: ZE15 (Bacillus subtilis) + ZR3 (Bacillussubtilis), T9: ZE11(Paenibacillus sp.), + ZE32 (Bacillus megaterium), T10: ZE11 (Paenibacillus sp.)+ZR3(Bacillus subtilis) and T11: ZE32 (Bacillus megaterium)+ZR3 (Bacillus subtilis). Means with different letters are significantly different at p≤0.05.
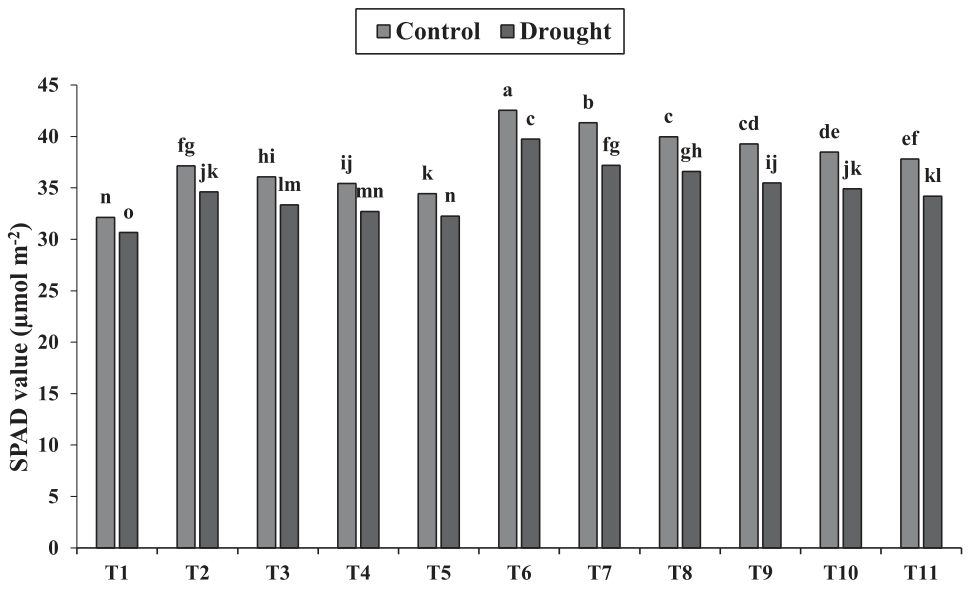
Fig. 6.
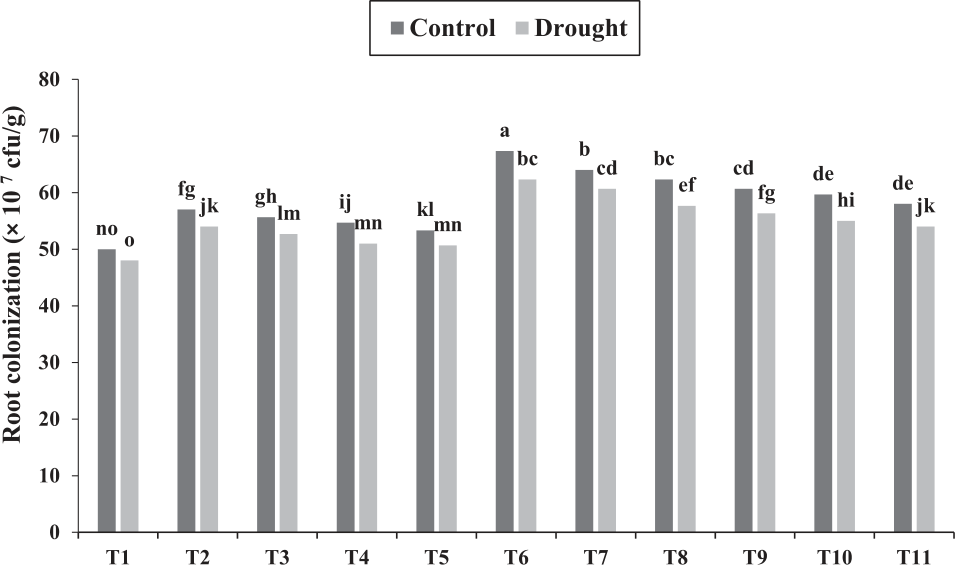
Potential of drought tolerant and IAA-producing rhizobacteria to improve root colonization of okra in jar trial T1: Control, T2: ZE15 (Bacillus subtilis), T3: ZE11(Paenibacillus sp.), T4: ZE32 (Bacillus megaterium), T5: ZR3(Bacillus subtilis), T6: ZE15 (Bacillus subtilis) +ZE11 (Paenibacillus sp.), T7: ZE15 (Bacillus subtilis) +ZE32 (Bacillus megaterium), T8: ZE15 (Bacillus subtilis) + ZR3 (Bacillussubtilis), T9: ZE11(Paenibacillus sp.), + ZE32 (Bacillus megaterium), T10: ZE11 (Paenibacillus sp.)+ZR3(Bacillus subtilis) and T11: ZE32 (Bacillus megaterium)+ZR3 (Bacillus subtilis). Means with different letters are significantly different at p≤0.05.
Improved Root Colonization of Okra with Drought-Tolerant IAA-Producing Rhizobacteria
The sole and co-inoculation effectiveness of bacterial strains on root colonization of okra plants in control and drought conditions are indicated in Fig. 6. Our results showed a significant decrease of 23% in root colonization in drought seedlings than well-watered seedlings. The bacterial strains applied in different treatments significantly improved root colonization compared with drought treatment. The results indicate that the combined application of the bacterial strains improved chlorophyll content more than the sole application. Among sole inoculations, strain ZE15 (Bacillus subtilis) (T2) had the highest increase of 12% compared to the un-inoculated control under drought conditions, followed by ZE11 (Paenibacillus sp.) (T3) with a 10% increase. As the result of co-inoculation of ZE11 (Paenibacillus sp.) and ZE15 (Bacillus subtilis) (T6) under drought conditions, the co-inoculation showed the most improvement. The improvement was 25% higher than the un-inoculated control under drought conditions. The subsequent treatment (T7) inoculated with ZE15 (Bacillus subtilis) + ZE32 (Bacillus megaterium) showed better results, where a 21% increase was recorded.
Discussion
Drought is a damaging climate extreme that has a detrimental impact on okra production worldwide [38]. Okra growth and yield are severely restricted by intermittent water deficit stress at regional and global scales [39]. Several bacterial strains pre-isolated and pre-characterized for their capacity to withstand PEG-induced osmotic stress were examined in this study. To determine how drought-tolerant strains responded to water deficit stress, drought-tolerant seeds were inoculated with drought-tolerant strains. Due to the limited availability of water, bacterial growth is negatively affected by water deficit stress, making drought-resistant bacteria an attractive alternative for dry climates [40]. It was found that Bacillus sp. ZE15 (Bacillus subtilis) and ZE32 (Bacillus megaterium) exhibited the highest growth rates, indicating that Bacillus sp. has essential roles to play in surviving adverse environmental conditions [41]. It was also found in our study that Enterobacter sp. was able to maintain high growth under osmotic stress, which led to them being drought-tolerant bacteria. Because of these findings, it is very likely that Paenibacillus sp. ZE11 is capable of colonizing dry soil effectively enough to colonize okra [42]. Seedlings inoculated with drought-tolerant strains of Bacillus subtilis, Paenibacillus sp., and Bacillus megaterium exhibited a faster increase in biomass than those inoculated with strains other than ZE15 (Bacillus subtilis). As a result, these strains’ growth-promoting properties are mainly determined by their ability to regulate 1-aminocyclopropane-1- carboxylate (ACC) deaminase activity and their ability to synthesize phytohormones in plants [43].
There has been evidence that the combination of PGPR and ACC deaminase activity when inoculated into plants can help lessen the effects of metabolic stress induced by ethylene on the growth of plants. PGPR is capable of cleaving the ethylene precursor ACC into ketobutyrate and ammonia, which may be the reason why it is capable of lowering ethylene concentration; consequently, the roots of plants can maintain their normal growth rate [44]. In the absence of water, the cleavage of the ACC by strains of Pseudomonas causes plants to produce low levels of ethylene, and the result was that plants inoculated with Pseudomonas strains significantly increased their root length, root and shoot fresh weight, and dry biomass in comparison to drought-stressed and non-stressed controls [45].
Water deficit stress’s physiological, biochemical, and molecular effects have profound consequences for plant growth on many levels [46]. A PGPR-based system can help increase a crop’s stress tolerance by promoting lateral root development, regulating photosynthetic capacities, and enhancing antioxidant capacity [47]. Because of PGPR-inoculation to crop seeds, it has been proven that the availability of water and nutrients in the soil has been improved. This allows plant growth to occur during drought periods [48]. The selection of the right PGPR strain is essential, as microbes can vary in their ability to withstand stress environments and effectively stimulate defense mechanisms in crops such as wheat and okra. [45]. In dry soil, osmotic stress may reduce the number of bacteria inoculated due to the physicochemical and biological properties of the soil [49]. Researchers have widely utilized them to improve crop performance in unfavorable conditions in recent years [50, 51]. The existence of Bacillus sp. as a biofertilizer is suggested by [52] since the bacteria are capable of producing more metabolites than other bacteria and are capable of forming spores. It is possible to increase crop yield and productivity by increasing the activity of ACC deaminase and EPS in arid climates with low enzyme activity [53, 54].
Despite the adverse effects of drought stress on both root morphology and growth parameters of okra, lack of inoculation significantly increased growth in uninoculated seedlings, whereas inoculated seedlings showed substantially better growth. It has been suggested that the benefits of PGPR to plant growth are attributed to its ability to solubilize nutrients, produce siderophores, and regulate critical hormones during water deficits [55, 56]. The results of this study are similar to those of [49], who reported that inoculating okra seedlings with bacteria tolerant of osmotic stress improved plant growth under water shortage conditions [57].
As reported by [41], Bacillus sp. is capable of colonizing dry soils and improving soil water potential by increasing aggregate stability, which can reduce the adverse effects of drought on plant growth. In addition to colonizing soils, Bacillus sp. can also reduce the damage done by drought on soil moisture [58]. Based on the results of the current study, inoculated seedlings exhibited increased shoot and root biomass because of long roots and shoots as well as the increased formation of lateral roots and root hairs, which assist plants in absorbing nutrients and water during droughts [59]. These bacterial strains also enhanced the growth promotion of non-pathogenic bacteria by combining them with ZE15 (Bacillus subtilis), ZE11 (Paenibacillus sp.), ZE32 (Bacillus megaterium), and ZR3 (Bacillus subtilis) as a consortium of microorganisms to make a synergistic growth promotion method. Recently, there has been a trend towards using multiple bacterial strains in conjunction with each other, which is more effective at stimulating crop growth and development than single bacteria [60, 61].
The success of the PGPR application lies in establishing a functional associative symbiosis in consortium formulations [62]. Evaluation of different combinations of bacterial inoculants is necessary for determining the most effective consortium to improve plant resistance to various stresses, such as drought [63]. Research shows that the application of PGPR to the bacterial community can have a significant effect. Several aspects of plant growth were investigated in this study including root length, dry weight, fresh weight, height, and microbial quantity. Control plants and inoculated plants had significantly different growth characteristics as drought stress increased, but inoculated plants’ growth characteristics improved significantly [64].
Conclusions
Consequently, our findings support that different bacterial strains have different response patterns to drought stress. Therefore, drought-tolerant inoculants are a valuable tool for enhancing the growth of okra under water-scarce conditions, as evidenced by our results. Inoculated plants of okra with the bacteria ZE15 (Bacillus subtilis), ZE11 (Peni-bacillus sp.), and ZE32 (Bacillus megaterium) showed high drought tolerance due to the preservation of leaf water status, which led to more pigments and more photosynthetic activity. As a result, the plants produced a more significant amount of biomass compared to the uninoculated controls. It has been suggested that the growth-promoting effects of PGPR can be attributed to the solubilization of nutrient molecules, the production of siderophore compounds, and the regulation of crucial hormones during drought conditions. Our study also demonstrated that okra seedlings inoculated with bacterial consortia tend to grow faster compared to those inoculated with individual strains of bacteria under water limitations. According to this study, drought-tolerant bacterial strains and their consortia are potentially valuable sources of biofertilizer for farmers in areas that experience a great deal of drought. The feasibility of using indigenous biofertilizers for dry land agriculture needs to be evaluated in further field trials to assess their potential use.
In the future, characterizing more bacterial strains with multiple growth-promoting traits, particularly those related to Indole acetic acid (IAA) production, should be a priority for inducing drought stress tolerance in specific crops. Research objectives should include evaluating IAA-producing bacteria under natural conditions and testing them in soils with diverse physicochemical properties across agroecological zones.

