

Introduction
Soil heavy metals (HMs) pollution is a serious environmental concern that is negatively affecting crop productivity, ecosystem health, and bio-diversity [1]. Heavy metals inhibit plant growth and development, and they also impose detrimental impacts on humans, animals, and plants [2]. Lead (Pb) is a serious HM, and its concentration in the environment continuously increases owing to increased industrialization, sewage sludge release, and fertilizer use [3]. A high amount of Pb found in daily-use vehicles’ acid batteries is released into the environment during recycling or disposal. Further, pipe, paint, and gasoline are the key sources of Pb release in the environment and its entry into the soil [4].
Lead toxicity negatively affects plant functioning, ranging from seed germination to final productivity. Lead toxicity negatively affects seed germination, root and shoot growth, and reduces water and nutrient uptake, significantly decreasing plant growth and productivity [5,6]. A high concentration of Pb reduces plant biomass production by decreasing chlorophyll (chl), plastoquinone, and carotenoid synthesis, photosynthetic rate, and damaging the photosynthetic apparatus [7,8]. Lead toxicity also causes reactive oxygen species (ROS) production, damaging proteins, lipids, and DNA, reducing biochemical and physiological activities [9]. Further, Pb toxicity also disturbs the organization of microtubules in meristem cells. It interferes with cell division in roots, which reduces root growth and causes a reduction in water and nutrient uptake [10]. A study on invasive plant species, including weeds, depicted that Pb toxicity caused stunted growth, chlorosis, blackening of roots, chloroplast ultrastructure distortion, electron transport obstruction, and inhabitation of Calvin cycle enzymes. Moreover, Pb toxicity also impairs the uptake of essential elements, induces CO2 deficiency due to stomatal closure, and reduces the uptake of water and nutrients, which causes a reduction in plant growth of invasive plant species [11].
Plants adopt different mechanisms to tolerate Pb toxicity. For instance, plants activate antioxidant defense systems that scavenge Pb-induced ROS production, and some plants also accumulate the Pb in roots and prevent the movement of Pb to shoots [12]. Further, Roots use Ca2+-permeable channels via the apoplastic route to absorb Pb from soil [13]. The Casparian strips block endodermis and restrict the further transport of Pb into plant shoots. Therefore, Pb accumulates in root cells [14]. Heavy metals inhibit plant growth and development. However, they also allow plants with higher tolerance to thrive on HM-polluted soils [15]. Different plant species have been found to colonize the HM-polluted soils efficiently [16]. Thus, it is vital to explore the mechanism of HM tolerance and competition amid the interacting species in response to HM-polluted soils [17]. Heavy metal-contaminated soils can be cleaned or restored using physical, chemical, or biological remediation methods. Phytoremediation is a novel method for eliminating environmental pollutants and remediating HM-polluted soils [18]. This method involves re-vegetating soil contaminated by harmful substances [19]. The phytoremediation process consists of the absorption of metals by plant roots and their translocation to shoots and leaves [20]. Different types of phytoremediation, including phytoextraction, phytofiltration, phytostabilization, phytodegradation, rhizosphere bioremediation, and phytovolatilization, are used globally to remediate HM polluted soils [18].
Different plant species like Brassica juncea, Eucalyptus urophylla, Vigna unguiculata, Zea mays, Myriophyllum brasiliense, Lycopersicon peruvianum, Solanum nigrum, Typha angustifolia, Cynodon dactylon, Ipomoea carnea, Bromus inermis, Dactylis glomerata, Triticum aestivum, Scirpus robustus, and Typha latifolia are being used globally to remediate HM polluted soils [21]. Weeds are among the most significant biological barriers to the sustainability of global agricultural production [22]. In contrast to crop species, weeds are typically more aggressive and frequently exhibit stress-resistant characteristics [23]. The present study hypothesized that weeds, being a more resistant plant species to stress, can thrive under Pb stress and serve as potential phytoremediation agents. The role of weeds as potential phytoremediation agents for Pb-polluted soils is rarely reported in the literature. Therefore, the present study aims to investigate the ability of different winter weeds (Chenopodium murale, Coronopus didymus, Avena fatua, Phalaris minor, and Medicago polymorpha) to thrive under Pb stress by exploring their biomass accumulation capability, gas exchange attributes, and antioxidant enzymes’ response, as well as exploring their phytoremediation potential by studying their Pb accumulation capacity and bioaccumulation factor. The objectives were achieved by analyzing the weeds’ capacity to accumulate metals and their physiological and biochemical responses under Pb toxicity.
Materials and Methods
Experimental Setup
A pot experiment was carried out to evaluate the phytoremediation potential of winter weeds against Pb toxicity. Seeds of five winter weed species were collected from Ayub Agricultural Research Institute Faisalabad, Pakistan. The pots, which had a capacity of 0.5 kg, were filled with soil to grow the weeds. The soil for filling the pots was collected from the Agronomic research area. The soil physio-chemical analysis was carried by as per Association of Official Analytical Chemists set protocols, and it was recognized as a clay loam with pH 7.82, organic matter 8.42 g kg-1, EC 0.94 dS m-1, available phosphorus 9.64 mg kg-1, exchangeable potassium 168 mg kg-1, and total nitrogen 0.33 g kg-1. Ten seeds of weed species were sown in each pot, and after germination, five plants were maintained in each pot after thinning.
Experimental Treatments
The study comprised of different levels of Pb stress control, 100 and 200 ppm, and different winter weeds Avena fatua, Phalaris minor, Coronopus didymus, Chenopodium murale, and Medicago polymorpha. The soil was spiked with PbSO4 by mixing the quantity of PbSO4 well as per treatment before pot filling to achieve the desired levels of Pb toxicity. Afterward, weed seeds were grown in each pot after the soil spiked with Pb.
Determination of Growth and Morphological Attributes
Thirty days old plants were harvested to measure the shoot and root lengths. Further, these plants were sun-dried for 4-5 days, followed by oven-dried (65℃) until constant weight to determine root and shoot dry weights.
Determination of Chlorophyll Contents
Chlorophyll contents (chl a and b) were measured by following the methods of Khaliq et al. [39]. Fresh leaves (0.1 g) from each pot were chopped and placed in falcon tubes containing 80% acetone and stored at 4°C overnight. Later, the absorbance was recorded at 663 and 645 nm to determine the concentration of chl a and b by using a spectrophotometer.
Gas Exchange Parameters
The standard procedure was followed to determine the photosynthetic rate, transpiration rate, internal CO2 concentration, and stomatal conductance. A photosynthesis system (Lci, 4225) was used to measure leaf gas exchange parameters. The flag leaf blade was placed under saturated PPFD conditions (>1200 L mol m-2 s-1) at a temperature of 25°C and CO2 concentration of 400 L mol mol-1 to determine gas exchange characteristics.
Antioxidants Enzymes
Catalase (CAT) activity was examined by following the method opted by Khaliq et al. [39]. The reaction mixture was made by mixing 50 µl enzyme crude extract with 100 ml of 10% hydrogen peroxide and 2.5 ml phosphate buffer (pH 7.0). The absorbance was noticed at a wavelength of 240 nm to measure the CAT activity. For determination of peroxidase activity, 100 ml plant extract was mixed with 0.32 ml of 5% guaiacol, 0.16 ml of 30% H2O2, 0.32 ml of 100 mM phosphate buffer, and 2.1 ml of ultrapure water to test peroxidase (POD) activity. The solution was immersed in cold water until it turned dark brown. The mixture was then placed in a cuvette to measure the POD activity by noticing the absorbance at 470 nm using a spectrophotometer.
To determine superoxide dismutase (SOD) activity, 100 µl EDTA was added to the reaction mixture. Each test tube contained 100 µl of Na2CO3, 100 µl of NBT, 1.5 ml of phosphate buffer, 200 µl of methionine in 100 µl of distilled water, and 100 µl of plant extracts. 100 µl riboflavin was pipetted into the reaction mixture. The enzymatic activity was then initiated by lightening the reaction mixture with two 15 W fluorescent lamps placed 30 cm apart. The reaction began in the presence of light, *significance at p<0.05, ** significance at p<0.01 which turned off after 10 minutes to stop the reaction. The non-irradiated mixture showed no color, and it was used as a blank, and absorbance was noted at 560 nm to determine SOD activity.
Table 1.
Values of F. calculated of various factors and their interactive effects from ANOVA
Pb Concentration in Shoot and Root (ppm)
The plant samples were taken and oven-dried to make the powder. After that, 0.5 g of crushed roots and shoots samples were taken in the conical flasks, and 3 ml HNO3 and 1 ml HClO4 were added to each flask and covered with foil for 8 hours. After that, the flask was uncovered and placed on the hot plate for 10 minutes until the color of the mixture turned colorless. Then, 10 ml of distilled water was added to each flask to avoid evaporation, and later, the volume was increased to 50 ml by adding more distilled water. The concentration of Pb in plant parts was determined by using an Atomic Absorption Spectrophotometer (Agilent Technologies, Santa Clara, CA, USA).
Bioaccumulation and Translocation Factors
Bioaccumulation factor determines the ability of any plant species to remediate the HM from the soil. The translocation factor defines the capacity of plants to translocate HM from root to shoot. Therefore, in the present study, the bioaccumulation and translocation factor of Pb were determined by using the methods of Alaboudi et al. [38].
Statistical Analysis
The recorded data was evaluated with SPSS statistical software using Fisher’s analysis of variance technique. Tukey’s HSD test at a 5% probability 5% was used to assess the significance between treatments mean. Moreover, figures were prepared in Sigma Plot 14.0 (SPSS Inc., Chicago, IL, USA), and the correlation matrix was drawn using R Studio 4.6.1 (R Studio, Boston, MA, USA).
Results
Plant Growth Morphological Attributes
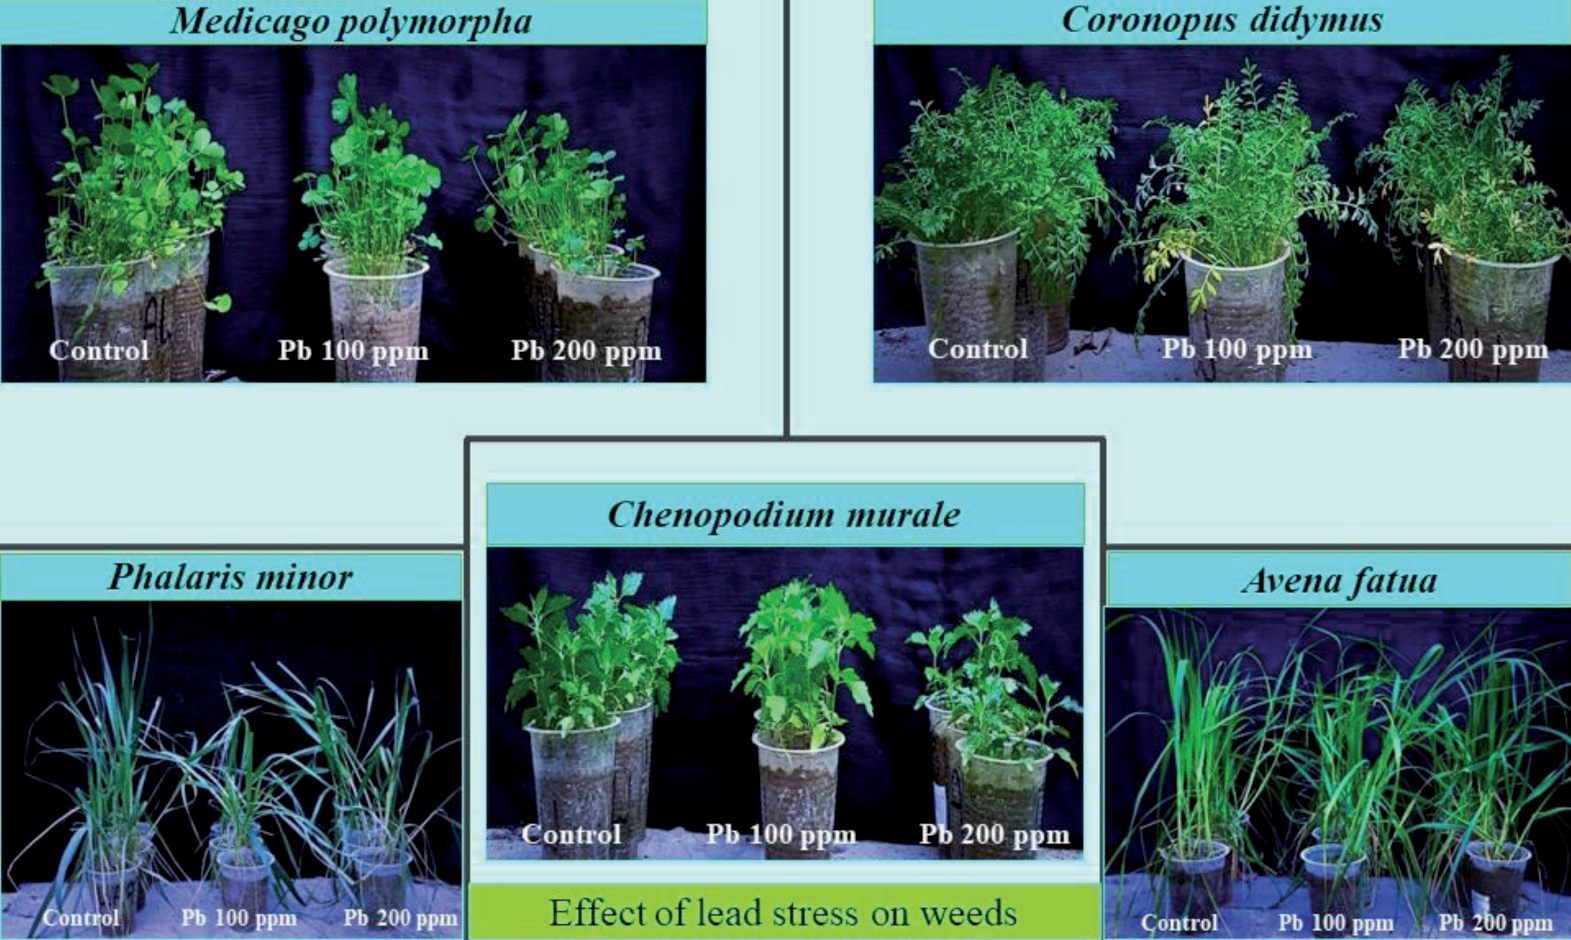
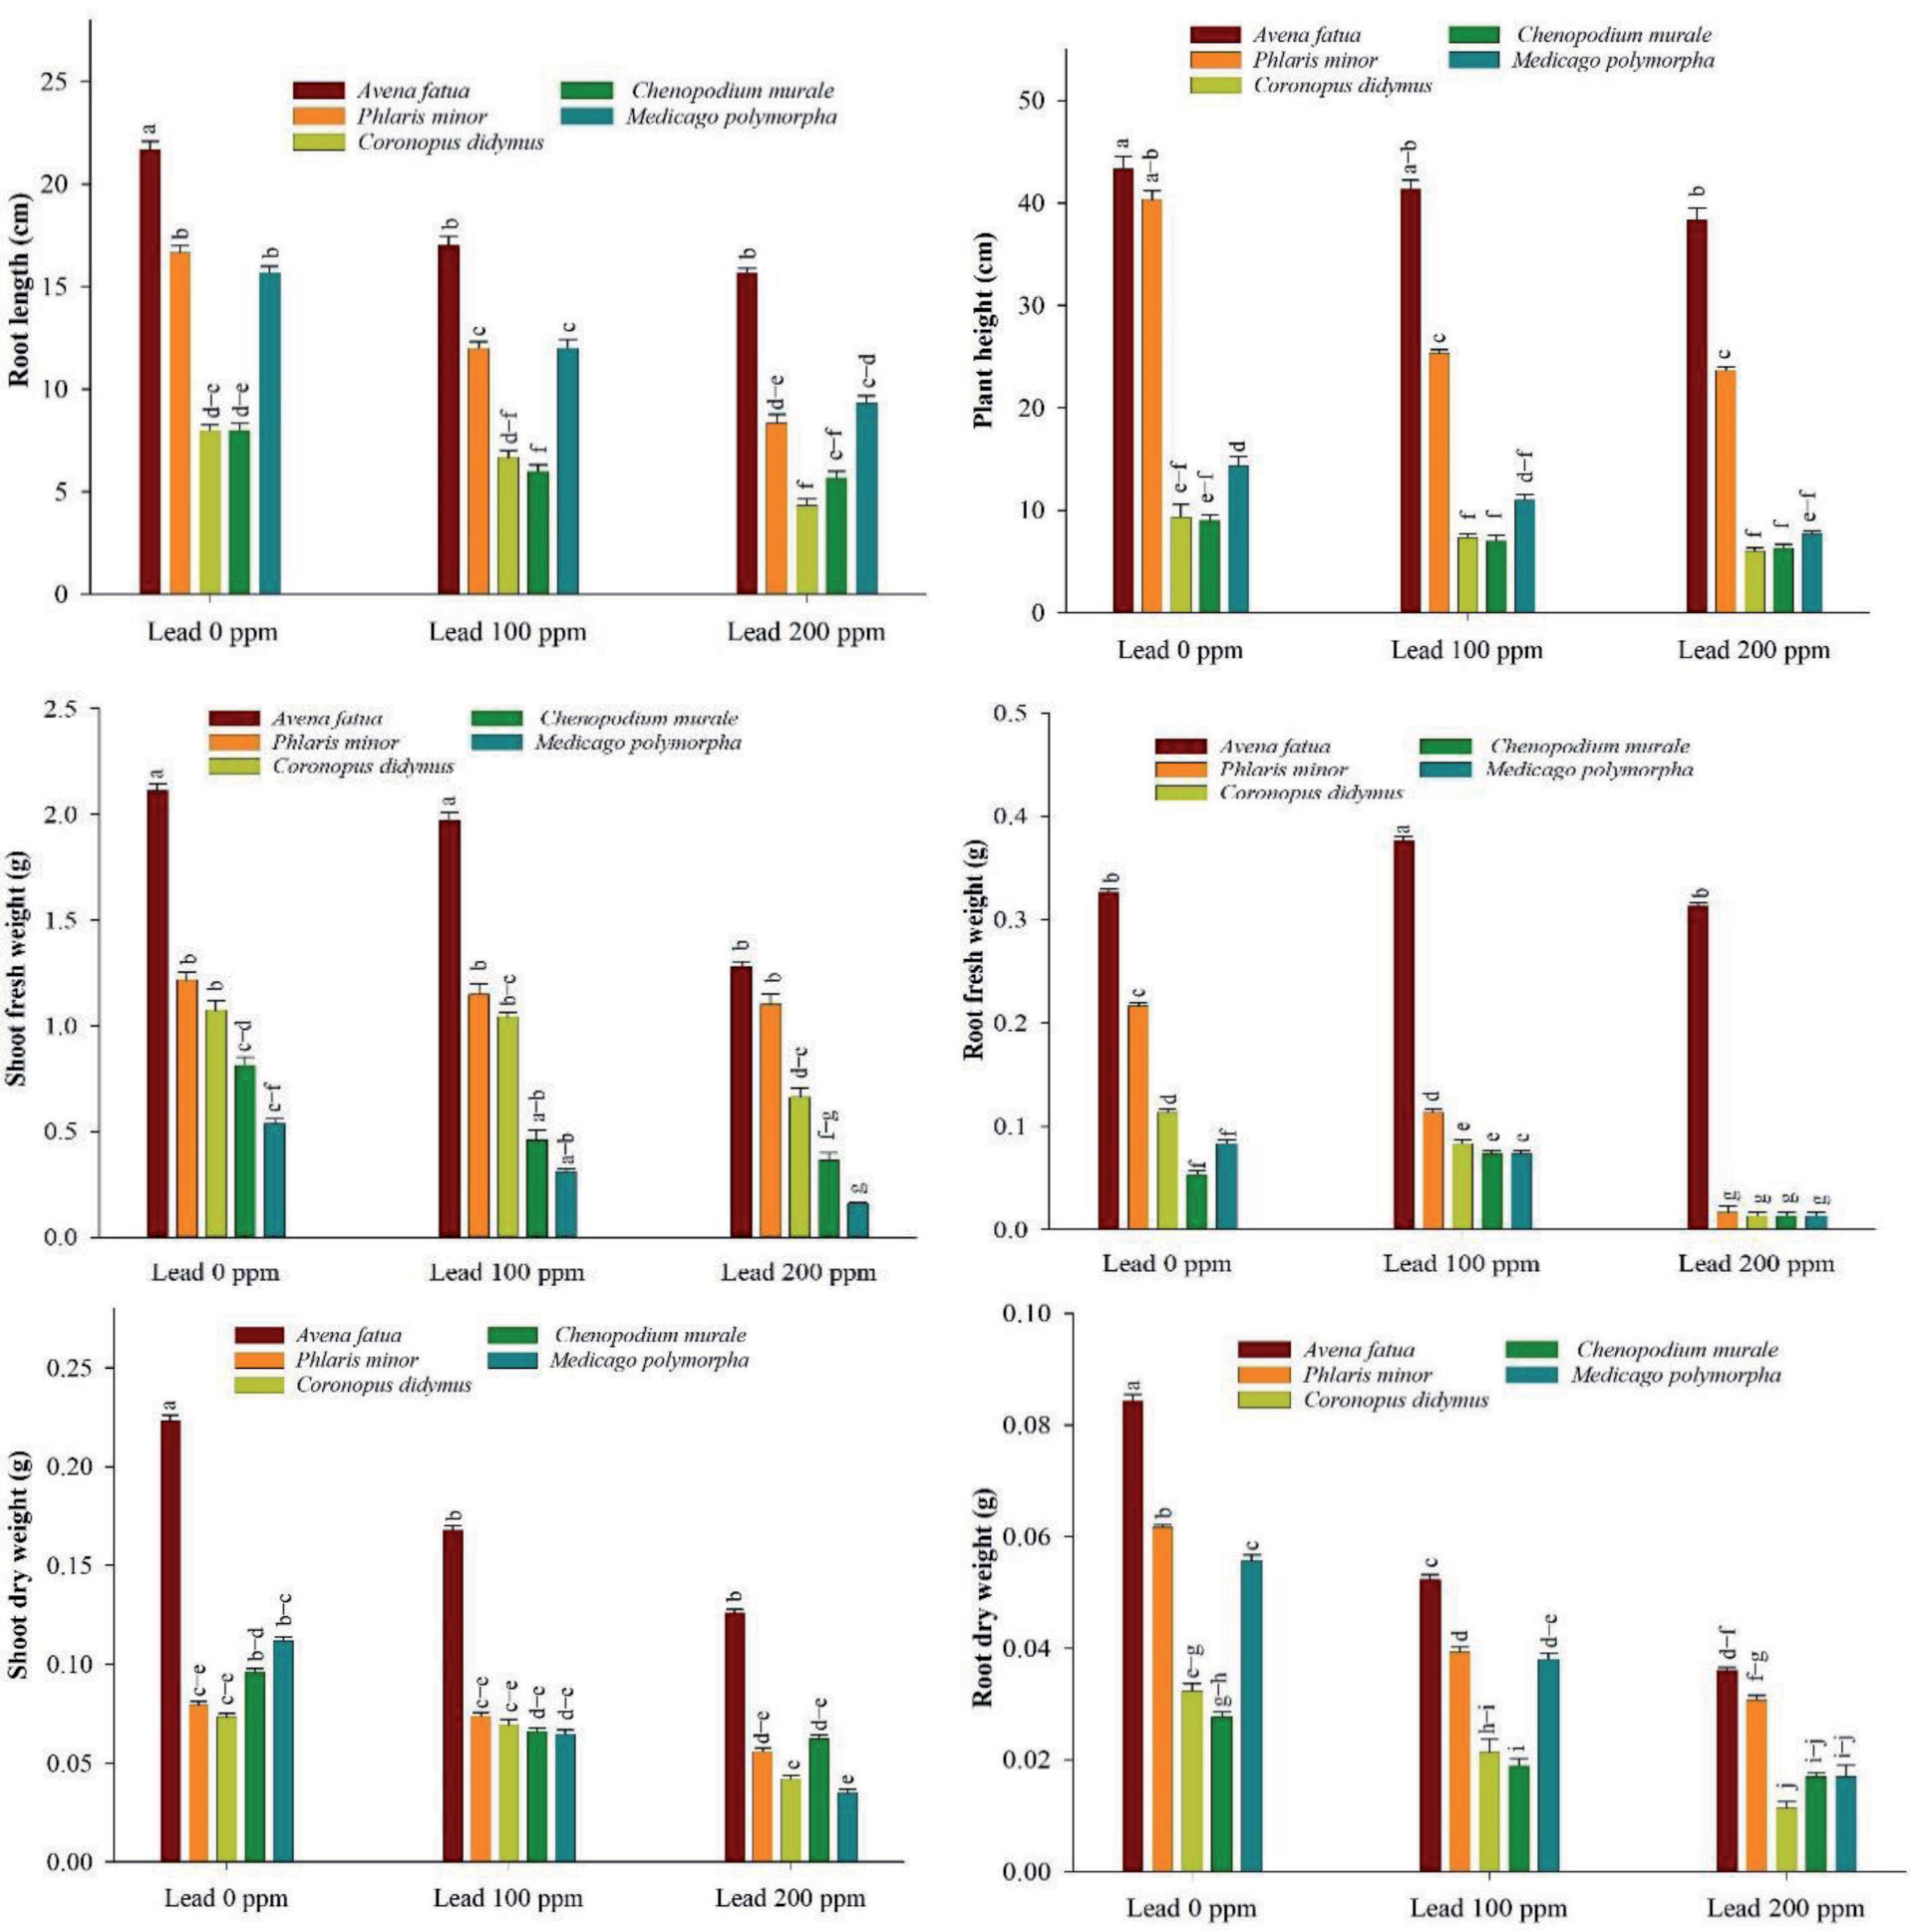
The interactive and main effects of various weeds and Pb concentration were found to be significant regarding plant morphological attributes (Table 1). The effect of two Pb concentrations on weed morphology is presented in Figure 1. The results indicated that Pb stress showed a significant (p<0.05) impact on the root length of different weeds (Figure 2). Root length was reduced by 27-50% due to severe Pb toxicity (200 ppm), while root length was decreased by 16-28% under 100 ppm Pb stress across all weeds (Figure 2). However, a minimum reduction in root length (11%) was noticed in Chenopodium murale plants, and this weed was found to be more tolerant under Pb toxicity. On the other hand, Phalaris minor was noticed as the most sensitive weed against Pb stress, and a maximum reduction in root length (50%) was observed in this weed under 200 ppm Pb stress (Figure 2).
Similarly, a significant (p < 0.05) interaction of Pb × weeds were recorded for the shoot length of different winter weeds. The utmost reduction (47%) in shoot length of Medicago polymorpha was recorded at the 200 ppm Pb level. In contrast, Chenopodium murale, Coronopus didymus, and Phalaris minor shoot lengths were reduced by 30%, 35%, and 41%, under 200 ppm Pb stress compared to control (Figure 2). Nonetheless, Avena fatua plants could tolerate the Pb toxicity, as they showed a minimum reduction (11%) in plant height under 200 ppm Pb stress as compared to the control.
Plant Biomass
Pb stress had a diminishing effect on the shoot dry weight of different winter weeds (Figure 2). Medicago polymorpha showed a reduction of 69% and 38% in shoot and root dry weight at 200 and 100 ppm Pb toxicity as compared to control (Figure 2). The Coronopus didymus and Phalaris minor showed the minimum decrease in shoot dry weight of 5% and 7% at 100 ppm Pb stress, while these weed species showed a reduction of 29% and 69% at 200 ppm Pb toxicity (Figure 2). In contrast, Coronopus didymus, Phalaris minor, and Avena fatua plants demonstrated the ability to withstand Pb toxicity, as evidenced by minimal reductions (3%, 5%, and 7%, respectively) in shoot fresh weight at the 100 ppm Pb level.
The different levels of Pb toxicity also had a significant impact on the root length of all the weeds. Avena fatua showed a higher tolerance to Pb toxicity, since they displayed the lowest reduction in root fresh weight of 15% and 4% at 100 ppm and 200 ppm Pb toxicity, respectively. On the other hand, Phalaris minor showed the highest reduction (47% and 92%) in root fresh weight at 100 and 200 ppm Pb levels. Coronopus didymus, Chenopodium murale, and Medicago polymorpha had intermediate levels of reduction in root fresh weight, with reductions of 26%, 38%, and 12% at 100 ppm Pb level and 88%, 75%, and 84% at 200 ppm Pb level (Figure 2).
Fig. 2.
Interactive effect of weeds and Pb toxicity on morphological and plant biomass attributes (plant height, root length, shoot dry weight, and root dry weight) of different winter weeds. The bar graph shows the mean and standard error of three replications. Bars with different letters differ significantly at 5% probability according to Tukey’s HSD test.
Leaf Gas Exchange Traits
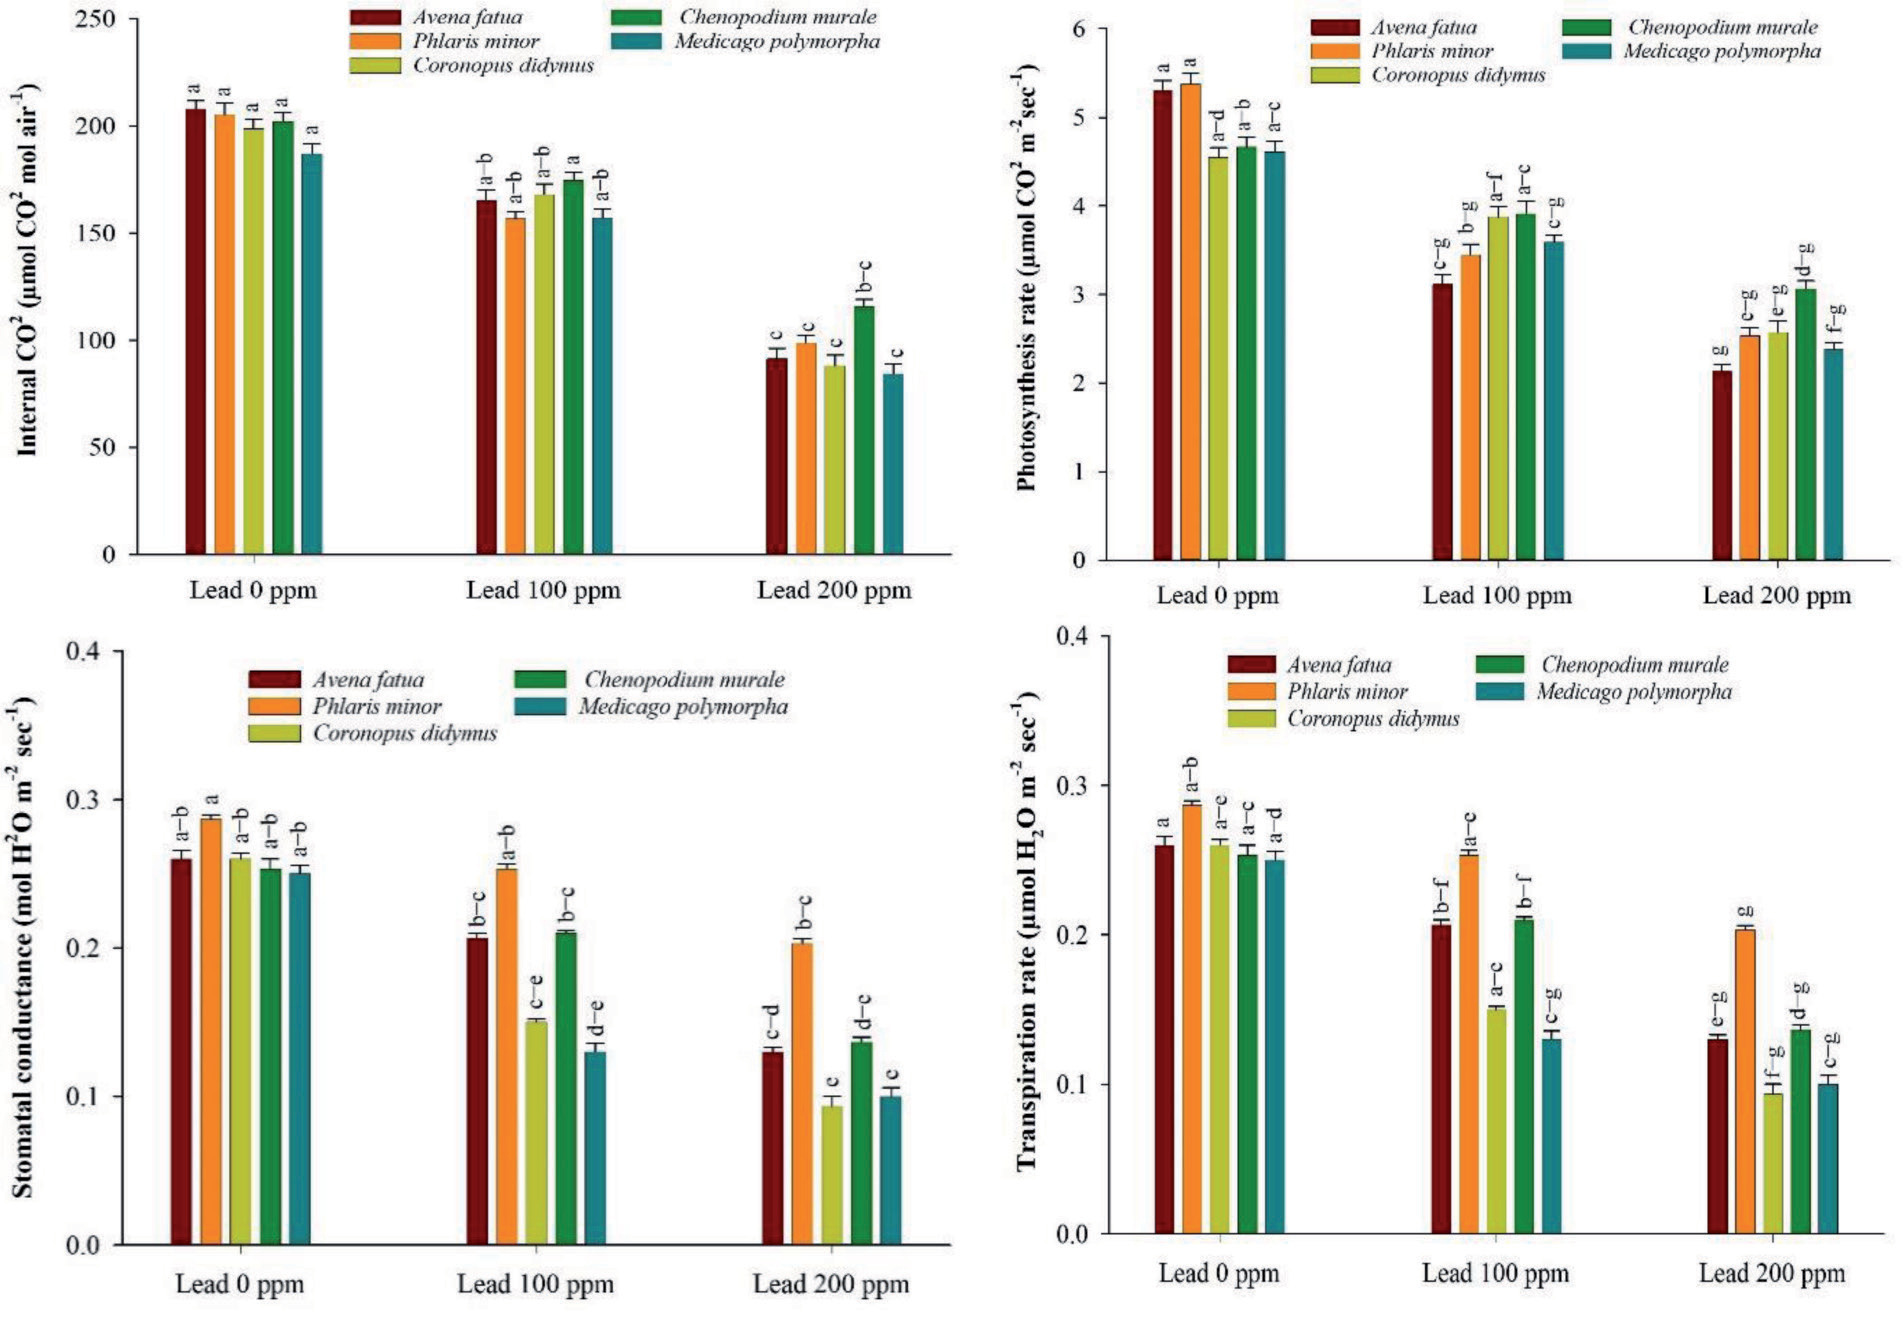
The photosynthetic rate of different weed species varied significantly among different Pb levels. Avena fatua showed a maximum reduction (60% and 40%) in photosynthetic rate under 100 and 200 ppm levels of Pb toxicity. In comparison, Phalaris minor showed a decrease of 36% and 53% photosynthetic rate at 100 and 200 ppm Pb (Figure 3). On the other hand, Coronopus didymus, Chenopodium murale, and Medicago polymorpha showed resistant ability with the minimum reduction of 5%, 16%, and 22% in photosynthetic rate under 100 ppm Pb level (Figure 3).
The results indicate that Avena fatua exhibited a 28% and 53% decrease in transpiration rate under 100 ppm and 200 ppm Pb stress, respectively. Phalaris minor demonstrated a 14% reduction in transpiration rate at 100 ppm Pb level and a 50% reduction at 200 ppm Pb level. In Coronopus didymus, a 21% reduction of transpiration rate was observed under 100 ppm Pb level and a 38% reduction at 200 ppm Pb level. Chenopodium murale showed an 11% reduction in transpiration rate under 100 ppm Pb level and a 38% reduction at 200 ppm Pb level. Finally, Medicago polymorpha exhibited a 33% reduction of transpiration rate under 100 ppm Pb level and a 29% reduction at 200 ppm Pb level. Among all weed species, Coronopus didymus, Chenopodium murale, and Medicago polymorpha showed the minimum photosynthetic rate (38%, 38%, and 29% than control) under 200 ppm Pb level. Interestingly, Medicago polymorpha recorded a maximum (33%) transpiration rate at 100 ppm Pb level (Figure 3).
The data showed that stomatal conductance varied significantly among different Pb levels and weed species. Avena fatua showed a 21% and 50% decrease in stomatal conductance at 100 and 200 ppm Pb levels, respectively. The weeds Phalaris minor, Chenopodium murale, and Coronopus didymus lowered their stomatal conductance by 12%, 17%, and 42% at 100 ppm Pb toxicity and by 29%, 46%, and 64% at 200 Pb toxicity level, respectively. However, Medicago polymorpha showed a maximum reduction of up to 48% at 100 ppm Pb level and a further reduction of 60% at 200 ppm Pb level (Figure 3). At the 200 ppm Pb level, internal CO2 concentration was reduced by 43-56% across all the observed weeds (Figure 3). The least reduction (14% less than the control) in internal CO2 concentration was recorded from Chenopodium murale plants that showed the ability to tolerate Pb toxicity. Conversely, Avena fatua showed a severe reduction (56% less than the control) in the internal CO2 concentration at the 200 ppm Pb level.
Photosynthetic Pigments
The study found that chl contents varied significantly (p<0.05) among different Pb levels. At the 200 ppm Pb toxicity, chl was decreased up to 10-36% across all the observed weeds, while chl-a content was decreased by 2-24% at 100 ppm Pb level. Avena fatua showed the highest reduction in chl-a and chl-b, up to 36% and 56% at 200 ppm Pb level (Figure 4). Phalaris minor, Coronopus didymus, Chenopodium murale, and Medicago polymorpha also showed reductions in chl-a under Pb stress, with the degree of reduction varying across the different Pb levels and weeds. However, Coronopus didymus plants showed relative tolerance by reducing only 10% chl-a contents at 200 ppm Pb toxicity level. On the other hand, Chenopodium murale plants recorded a minimum reduction (14%) of chl-b at the 100 ppm Pb level compared to the control. Furthermore, the chl-b of Chenopodium murale, Phalaris minor, and Medicago polymorpha plants was reduced by 43%, 52%, and 55%, respectively, at higher toxicity levels compared to the control. The findings suggest that different weeds have varying phytoremediation potential against Pb stress on chl (a and b) contents, indicating that different weed species behave differently. However, some species, like Coronopus didymus and Chenopodium murale, are more tolerant to Pb toxicity and may be better suited for phytoremediation efforts in Pb-contaminated environments (Figure 4).
Fig. 4.
Chl contents (a, b) exhibited by different winter weeds under Pb toxicity. The bar graph shows mean and standard error of three replications. Bars with different letters differ significantly at 5% probability, according to Tukey’s HSD test.
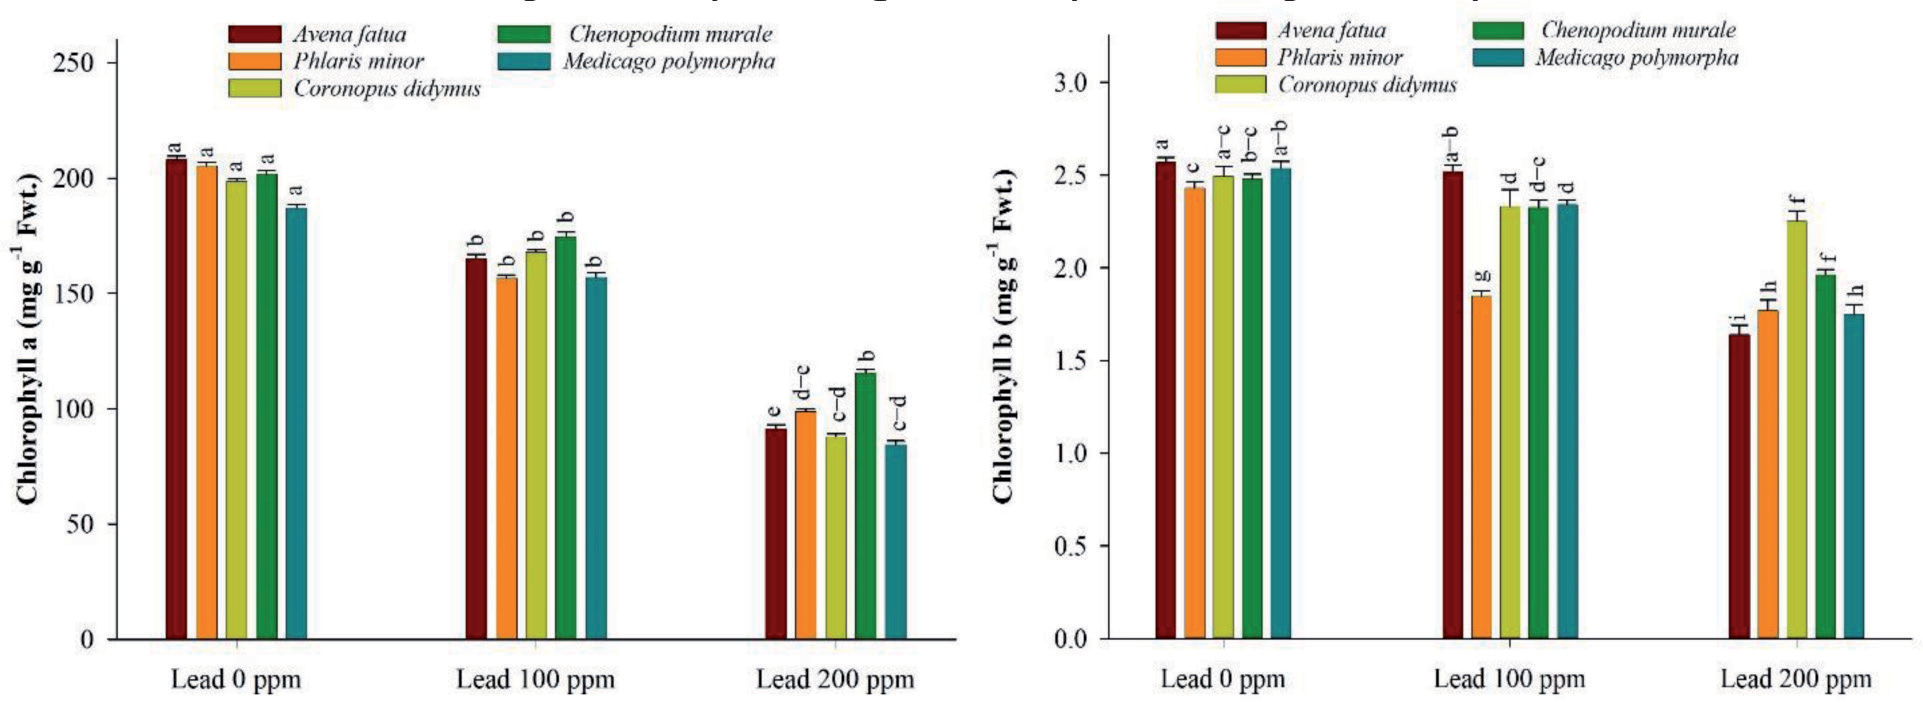
Fig. 5.
Interactive effect of weeds and Pb toxicity on photosynthetic attributes (internal CO2 concentration, photosynthesis rate, stomatal conductance, and transpiration rate) of different winter weeds. The bar graph shows mean and standard error of three replications. Bars with different letters differ significantly at 5% probability according to Tukey’s HSD test.
Antioxidant Activities
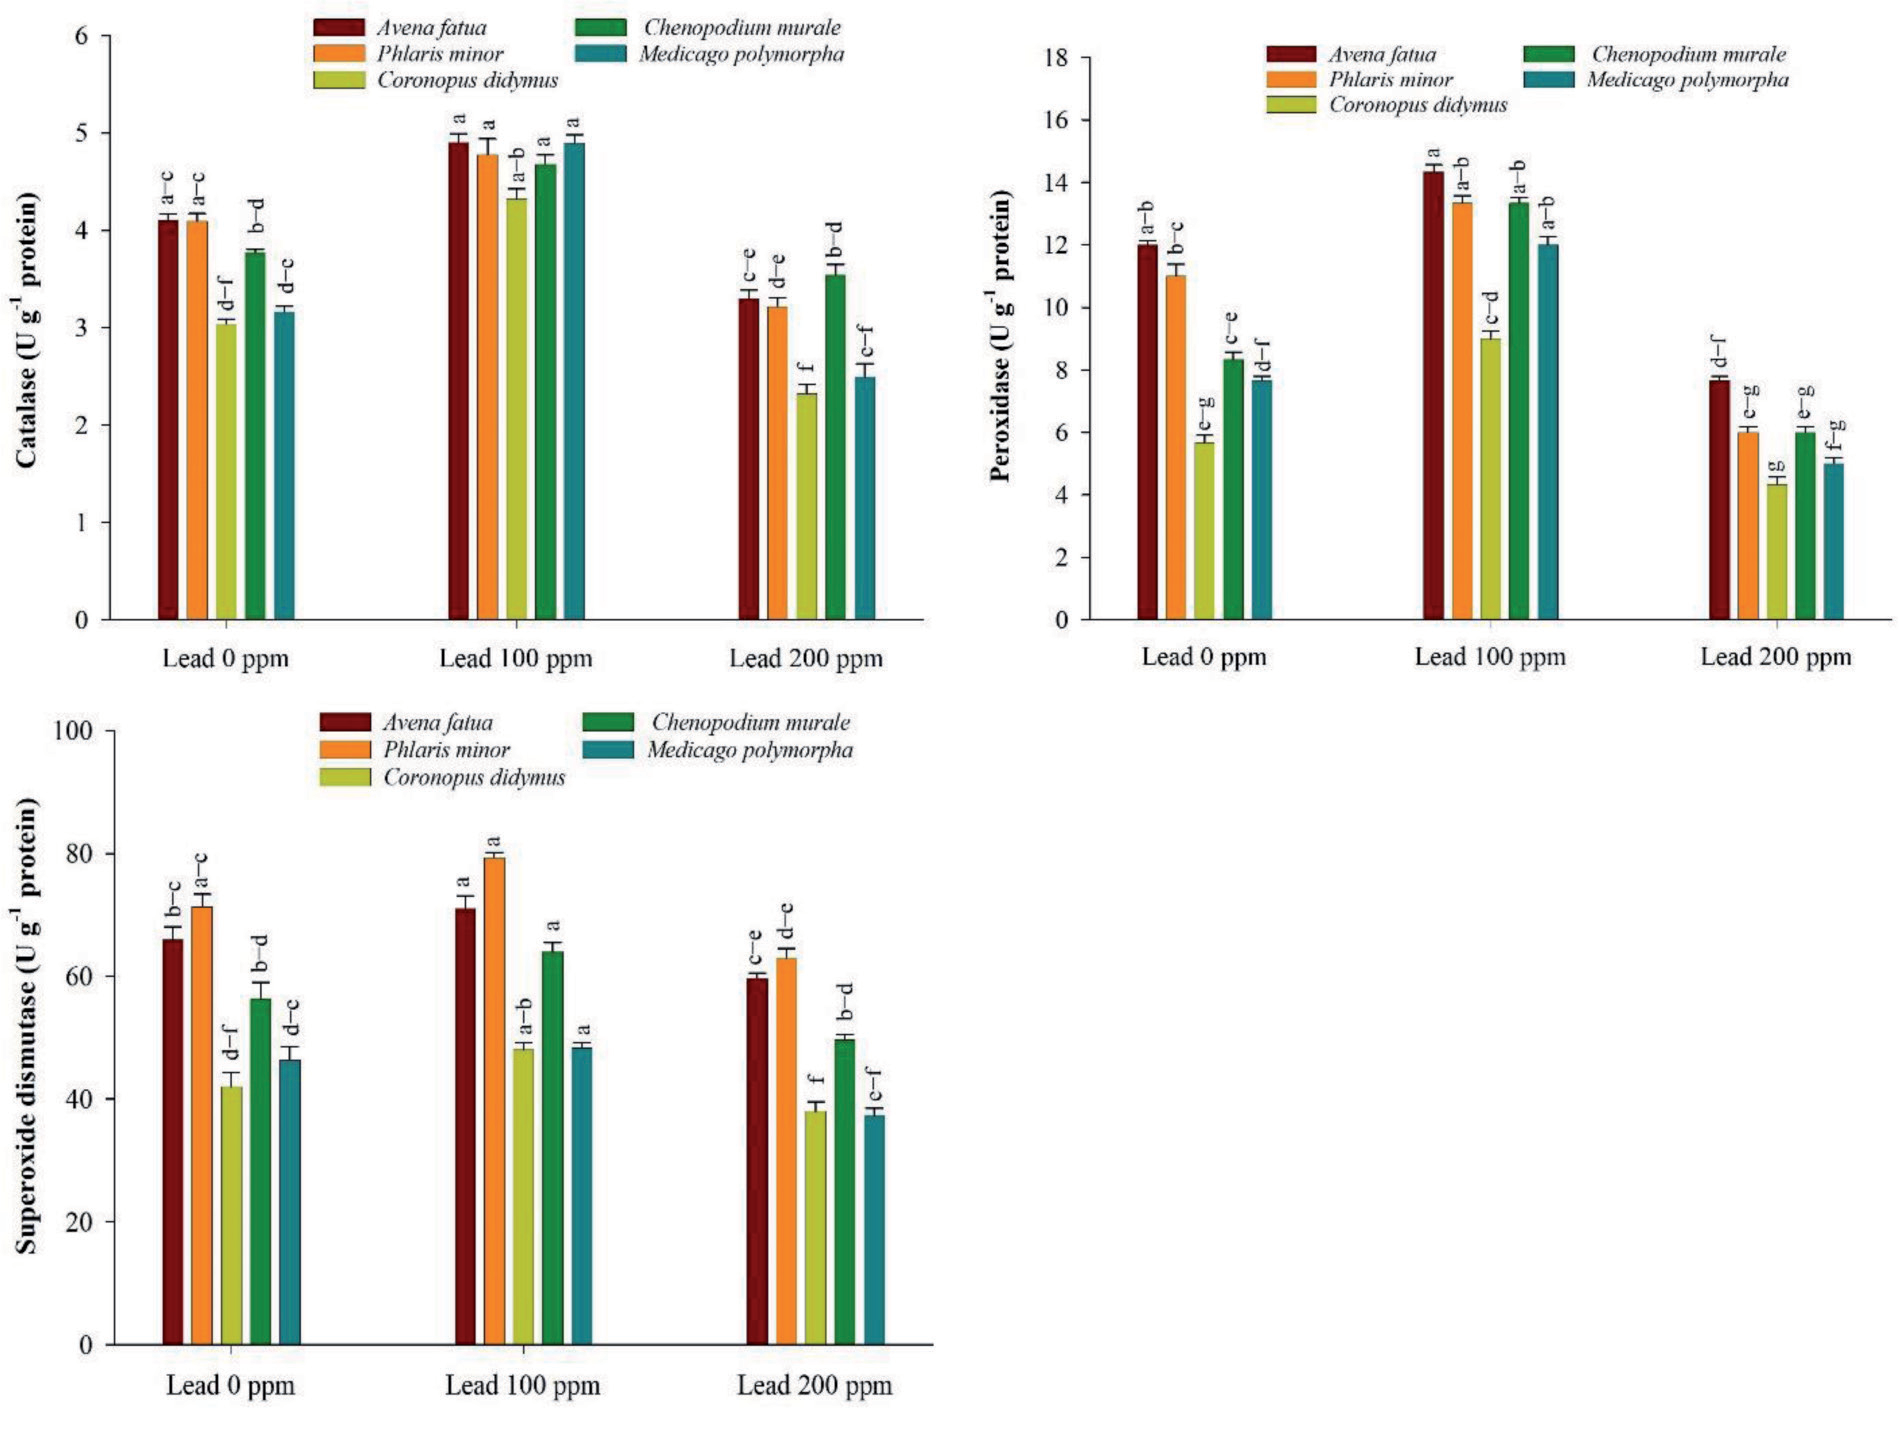
The activities of different enzymes (SOD, POD, CAT) of studied weeds were affected differently depending on the Pb toxicity level. At 100 ppm Pb level, the maximum increase (14%) in SOD activities was observed in Coronopus didymus and Chenopodium murale followed by Phalaris minor (11%), Avena fatua (8%) and Medicago polymorpha (4%). Whereas the Medicago polymorpha and Coronopus didymus showed the maximum CAT activities (55% and 42%, respectively) under 100 ppm Pb toxicity, followed by Chenopodium murale (17%) and Phalaris minor (24%) (Figure 5). Similarly, the POD activity was enhanced (19-60%) at 100 ppm Pb level and decreased to a lesser extent (24-35%) across all weeds at 200 ppm Pb level. In Chenopodium murale, the maximum (60%) POD activity was recorded at 100 ppm Pb level. However, due to high Pb toxicity, Phalaris minor showed a minimum reduction (45% less than the control) in POD activity at a Pb concentration of 200 ppm (Figure 5). Similarly, the highest reduction in SOD (19%) was observed from Medicago polymorpha followed by Coronopus didymus and Chenopodium murale at 10.5% and 12%, respectively, at 200 ppm toxic level. Phalaris minor showed a 12% reduction in SOD content, while Avena fatua showed a decrease of 10%. Further, the CAT contents were decreased by 24% and 21% at 200 ppm Pb toxicity in Coronopus didymus and Phalaris minor, respectively, compared to control. Moreover, Medicago polymorpha and Chenopodium murale showed a decrease of 21% and 6%, respectively. These results suggested that Pb toxicity negatively affected the enzymatic activities in all the weed species. However, the enhancement of SOD, POD, and CAT contents at lower levels of Pb toxicity showed the defense mechanism to protect the plant from oxidative stress (Figure 5).
Pb Concentration in Plants
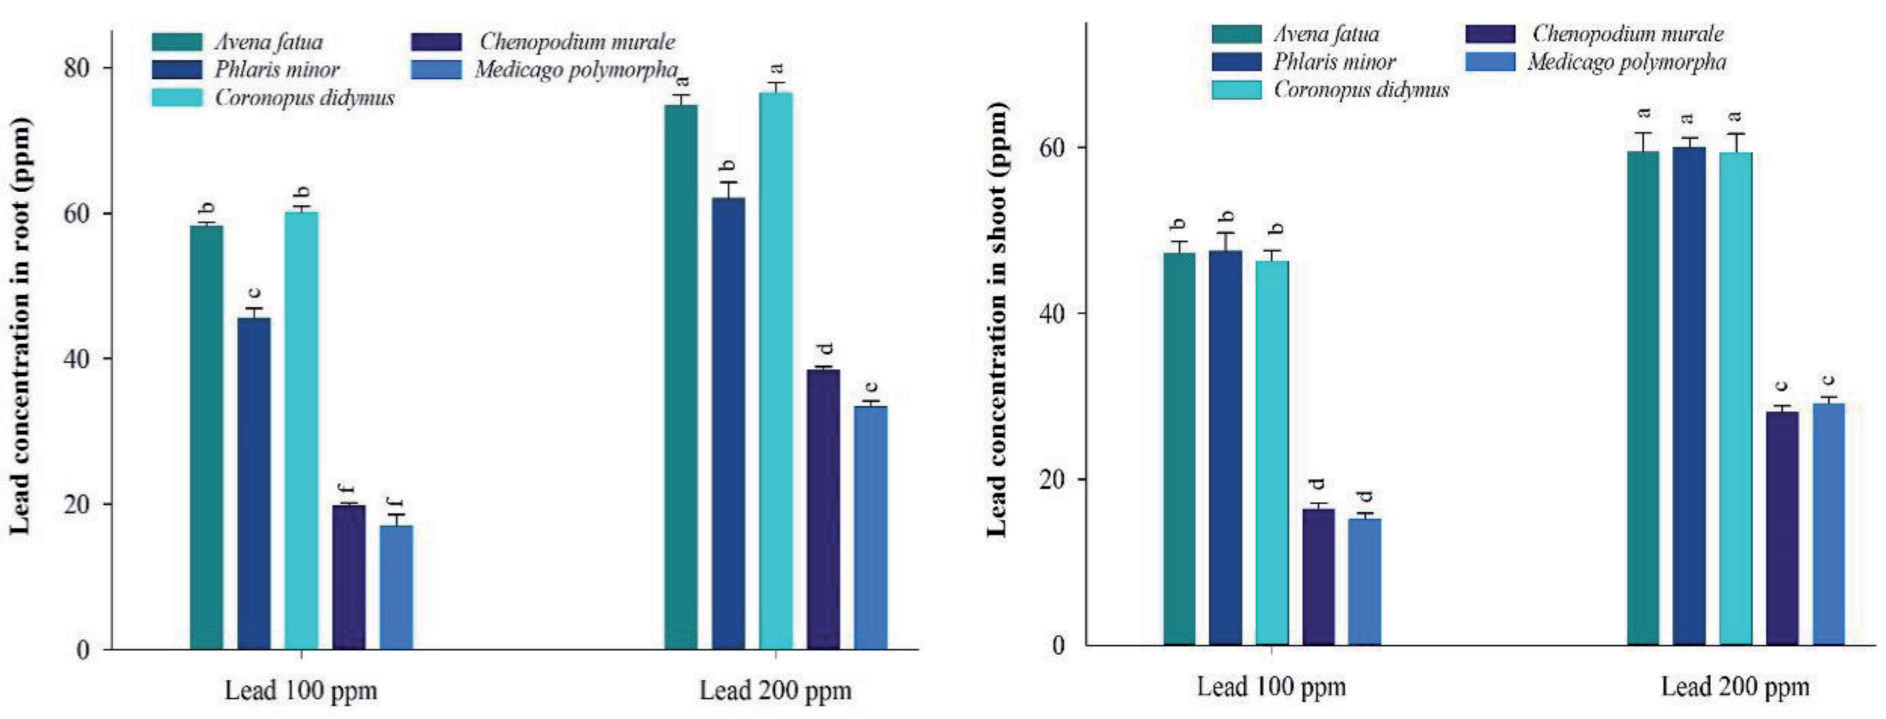
Two weed species, including Avena fatua and Coronopus didymus were more efficient in up-taking Pb than Phalaris minor at 100 ppm Pb level. However, Pb concentration in the shoots and roots of these three weed species were the same at 200 ppm Pb level. Further, Chenopodium murale and Medicago polymorpha proved less efficient in the uptake of Pb at both toxic levels (100 and 200 ppm Pb) (Figure 6).
Bioaccumulation and Translocation Factor (TF)
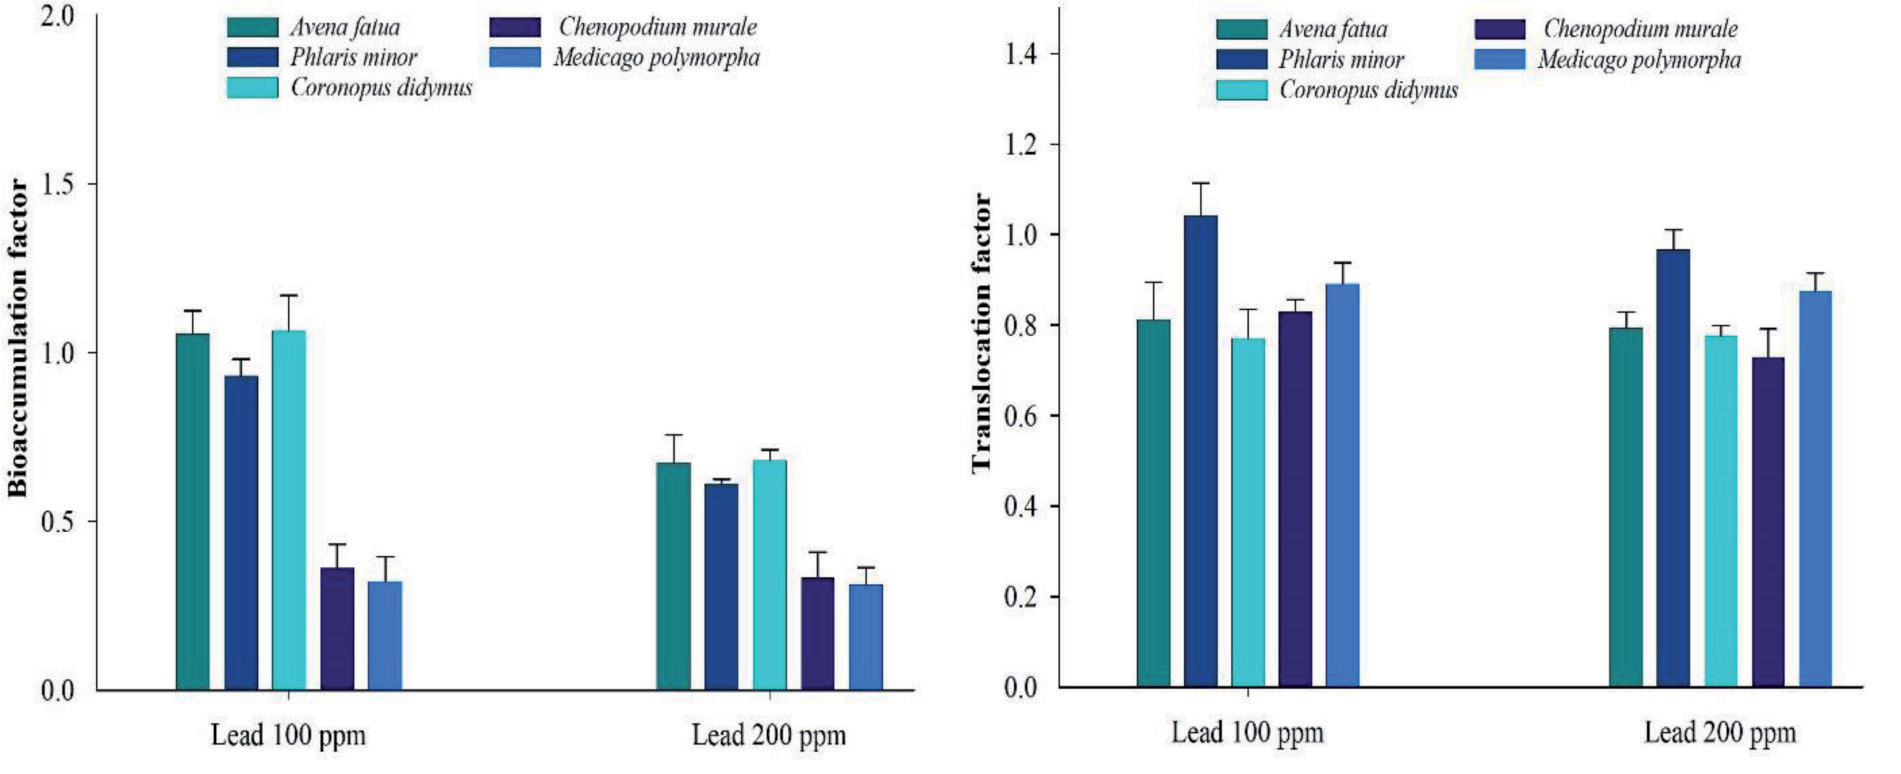
In the present study, Avena fatua and Coronopus didymus depicted a bio-accumulation factor of more than 1 at 100 ppm Pb level. Hence, these two weed species can be regarded as accumulators of Pb. Nonetheless, the other weed species could not maintain this capability at 200 ppm Pb level and showed ≤1 value of bioaccumulation; hence, those can be considered excluders of Pb (Figure 7). The translocation factor determines the ability of the plant to translocate the HM efficiently from root to shoot. Species depicting a value of TF ≥ 1 are considered efficient translocators of HM (Ang et al., 2023). The results of the present study revealed that Phalaris minor was more efficient in trans-locating Pb from its root to shoot. However, other weed species confined more Pb in roots than shoots (Figure 7).
Correlation Matrix
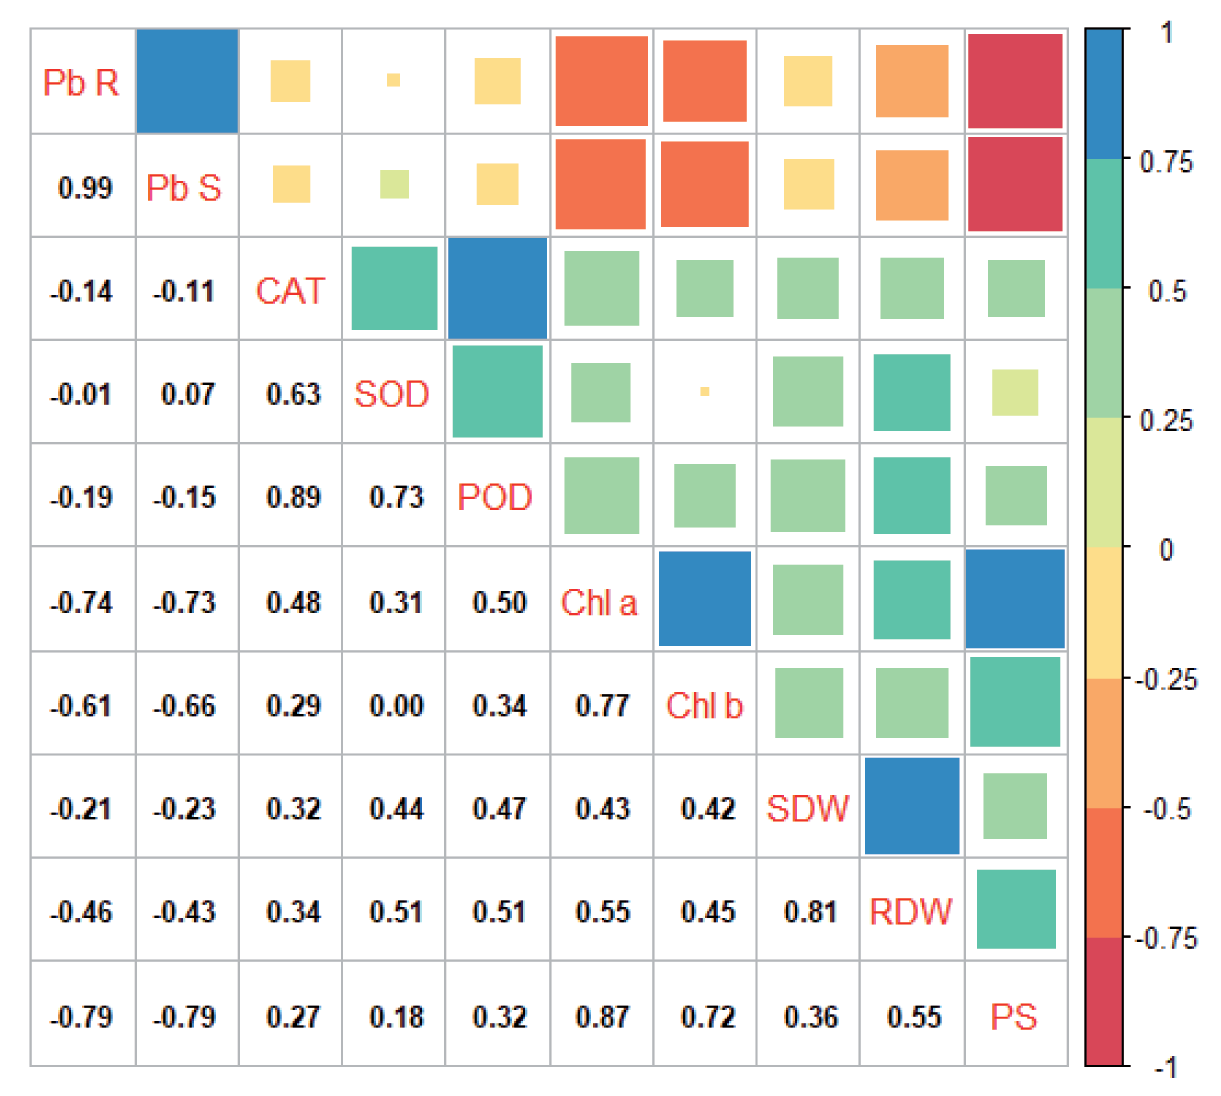
The correlation matrix showed that chl contents and photosynthesis rates were negatively correlated with Pb toxicity (Figure 8). Antioxidant production was increased to protect the plant seedlings from Pb-caused cellular damage. Hence, the antioxidant elucidated a positive correlation between chl contents and the plant biomass (Figure 8). The root and shoot dry biomass were negatively correlated with Pb contents in plants; however, root biomass showed a more negative correlation. Chlorophyll a content showed a positive correlation with antioxidants, owing to the cellular protection of these enzymes.
Discussion
Plants are subjected to various abiotic and biotic stressors that negatively affect their growth and development. Heavy metal toxicity is one of the most common and serious abiotic stresses, negatively impacting crop growth and development [24]. Pb toxicity is a serious HM that negatively affects plant growth and development by altering physiological and biochemical functions [9]. Metal removal techniques that are now in use are typically costly, damaging, labour-intensive, and result in additional issues. Comparatively, phytoremediation is an effective, economical, environment-friendly, and efficient method to treat HM-polluted soils [25].
Fig. 8.
Correlation matrix of different parameters under study. Pb S: Lead concentration in shoot, Pb R: Lead concentration in root, Chl a: Chl a, Chl b: Chl b, SDW: Seedling dry weight, RDW: Root dry weight, PS: Rate of photosynthesis.
Because of their innate resistance capacity and lack of appropriateness as fodder, wild weeds are excellent for phytoremediation purposes. Weeds are the most appropriate and effective way to combat the issues associated with HM pollution [26]. Different weeds respond differently to Pb stress; each weed showed different phytoremediation potential. Maximum morphological growth was observed in Avena fatua, and Coronopus didymus recorded minimum photosynthesis compared to other weeds. In the present study, Pb stress significantly reduced root and shoot growth and biomass production, possibly due to restricted cell divisions, photosynthetic efficiency, antioxidant activities, and chl synthesis [27-29].
Lead toxicity has a negative impact on the photosynthetic process. In the present study, Pb toxicity seriously reduced the photosynthetic rate and leaf gas exchange characteristics. Lead toxicity negatively affects chloroplast ultra-structure, restricts chl, plastoquinone, and carotenoid synthesis, and obstructs electron transport, decreases Calvin cycle enzyme activity and stomatal closure, thereby causing a reduction in the photosynthetic rate of weeds [30,31]. Besides this, Pb stress also reduces the stomata conductance, induces oxidative stress, and decreases the activity of ribulose-1,5-bisphosphate carboxylase/oxygenase, which hinders the photosynthesis and subsequent dry matter production in plants [31,32].
Different weeds respond differently to Pb stress in their photosynthetic rate; maximum photosynthesis was observed in Chenopodium murale, and minimum photosynthesis was recorded by Avena fatua compared to other weeds. In the present study, Pb stress decreased the stomata conductance and internal CO2 concentration, which is consistent with the findings of Zhou et al. [30]; they also found that Pb stress seriously decreased the stomata conductance and internal CO2 concentration. Lead toxicity seriously decreased the biomass and chl synthesis in all the weeds. Pb stress prevents chl production by preventing plants from absorbing vital nutrients like magnesium and iron. Due to its affinity for protein N- and S-ligands, it damages photosynthetic machinery. Plants exposed to Pb experience enhanced chlorophyllase activity, which accelerates chl breakdown, thus resulting in a substantial decrease in chl synthesis [31]. Further, Pb also interferes with photon electron transit and inhibits protochlorophyllide reductase activity, thus resulting in a marked decrease in chl synthesis [33].
The present study showed that Pb stress decreased the chl content of weeds, And Different weeds respond differently to Pb stress in their chl contents. Maximum chl content was observed in Chenopodium murale, and minimum photosynthesis was recorded by tooth burclover compared to other weeds. Our findings are in accordance with those of Hou et al. [34], who found that plants’ chl decreased as Pb concentration increased. The present study showed that Pb stress increased the different antioxidants like CAT, POD, and SOD of weeds, and with increasing concentration of Pb, these antioxidants were decreased. These findings are consistent with the findings of El-Mahrouk et al. [28]; they observed that CAT, POD, and SOD activities initially increased with rising concentrations of Pb stress, but additional increases in Pb stress caused a reduction in antioxidant activities. SOD, CAT, and POD activities considerably increased in Pb-treated plants compared to untreated controls, indicating the activation of numerous defense mechanisms to detoxify the metal-induced phytotoxicity [35] successfully. Different weeds respond differently to antioxidant activities under Pb toxicity.
The two most significant aspects are the total intake of HM from the analyzed soils and their elimination through the harvested biomass of the tested plants. Plant species can have varying propensities for metal uptake in their various parts. Numerous soil variables, such as pH, clay content, cation exchange capacity, nutrient balance, soil moisture, redox potential, organic matter, concentrations of other trace elements in soil, and soil temperature, have an impact on the uptake and accumulation of HM through plants [36]. The present study showed that Pb stress increased the soil, roots, and shoots Pb concentration, and its concentration was lower in stressful plants than in unstressed plants. Different weeds respond differently to Pb stress in their concentration. Each weed showed different phytoremediation potential, and the maximum accumulation potential of Pb was observed in Chenopodium murale. The minimum accumulation potential of Pb was recorded by tooth burclover than other weeds. The present results align with Chanu and Gupta [37], who explained that different plants have different potentials for phytoremediation. Ipomea has great potential for phytoremediation and exhibits high Pb accumulation, which was first found in the root and then in the stem and leaves.
Coronopus didymus has a remarkable capacity to absorb Pb, particularly in the roots. The migration of potential toxins like Pb enter and disrupt the food chain, which is reduced because it is a wild, undesirable plant species. As a result, Coronopus didymus has become a novel wild plant species that can be effectively exploited in the future to clean up Pb-contaminated soils [33]. Furthermore, the Pb content in the plant roots was roughly higher than that in the shoots, likely because roots are the main locations for metal outbursts that enable the plant to overcome Pb toxicity effectively. Bioaccumulation factors can explain the potential of any plant to be the accumulator of HM. In the present study, Avena fatua and Coronopus didymus depicted a bioaccumulation value of more than 1. Hence, these were the potential accumulators of Pb, as illustrated in other research studies [38]. The translocation factor depicts the potential of any plant to translocate HM fraction from root to shoot, and its value of more than 1 shows that the plant is efficient in translocating HM from root to shoot [38]. Results of the present study show that Phalaris minor was more efficient in translocating Pb to shoot; nonetheless, other weeds stored more Pb in their roots than shoots.
Conclusions
The present study focused on the performance of Avena fatua, Phalaris minor, Coronopus didymus, Chenopodium murale, and Medicago polymorpha under Pb stress. Plant biomass, antioxidant activity, chl contents, and gas exchange attributes under Pb stress depicted that these weeds were able to survive the higher levels of Pb. Further, Avena fatua, Phalaris minor, and Coronopus didymus accumulated more Pb in their body parts than the other two weeds. Bio-accumulation of Avena fatua and Coronopus didymus was more than 1; hence, it depicts their potential for being used as phytoremediation plants. It can be concluded that these weeds can thrive under Pb toxicity, and some possess the potential for phytoremediation. The ease of cultivating these weeds facilitates the phytoremediation procedure. Weeds accumulate high concentrations of Pb from contaminated soil and grow rapidly, making them an economical and environmentally favourable method. Nonetheless, certain logistical factors must be taken into account, including costs associated with cultivation, maintenance, and harvesting. It is necessary to develop harvesting and processing techniques for Pb-contaminated biomass that are both efficient and economical. Additional research could explore various weed-based Pb phytoremediation strategies in greater depth. Perform field experiments to evaluate the efficacy of Coronamus didymus and Avena fatua in Pb-contaminated environments. Determine the genes and enzymes that are involved in the uptake and transport of Pb by these weeds.

