


Introduction
Abiotic stress such as water deficit stress is the major factor that diminishes crop growth to a greater extent about 50% globally [1]. Salinity and water deficit stress are two common adverse ecological issues that affect the growth and yield of crops and are considered primary factors to reduce agricultural yield and production [2]. Water deficit stress is an important factor that causes a reduction in plant yield. Water deficit stress has major adverse effects on the plant such as diminishing crop yield and production, limiting water resources, and decreasing WUE [3]. The major cause of the water deficit is less rainfall and more evapotranspiration due to poor arrangements of water resources [4].
Areas in Pakistan affected by severe water deficit stress are Sindh and Baluchistan provinces [5]. Some parts of Southern Punjab are also affected by moderate water deficit stress. From 1964-2007, a decline of about 10% in crop yield occurred due to a shortage of water [6]. In Pakistan, about 3.5 m ha area is non-irrigated which is highly prone to water deficit stress. In Punjab, almost 10 districts are affected by water deficit stress [5]. In Sindh, 1.973 m ha of agricultural land is under water deficit stress causing a decrease in crop yield and cultivated area in Pakistan. Given present demographic examples and future development estimates, water deficit stress may affect up to 60% of the global population by 2025 [5]. Water deficit stress is a climatological word also known as the period of substantial rainfall and water loss condition. Water deficit conditions reduce seed germination and plant growth [7]. Water stress affects plant health by decreasing leaf size, diminishing crop yield, stem elongation, amount of cell division, and root propagation [8]. Water scarcity is also known as drought stress, and it influences the development and production of quinoa.
Silicon exists as a beneficial component in soil and has a significant role in decreasing drought stress in crops. For higher plants, it is not a crucial element. Si exists as the 2nd highly rich component on the earth’s surface [9]. In areas of arid and semi-arid, to enhance the production of quinoa, silicon is considered the most accessible amendment for this problem [10]. It helps the plant to overcome water stress-associated effects. Silicon can bring numerous modifications in plant uptake devoid of being consumed by natural factors [11]. Si can maintain crop yield and growth even in stressful conditions like biotic and abiotic stresses. It promotes water and solute transportation mechanisms and enhances photosynthetic activity [12].
The outer layers of cells, membrane pores, and interstitial gaps all contain silica in significant quantities. Both over and below the cuticular sections, it builds up. Numerous Si-containing agricultural plants have been studied to determine the importance of silica therapy to plant development, physical condition, and strength [13]. According to research outcomes, rice can be more resistant to both biological and physiological challenges when silicon is provided in appropriate amounts to crops [14].
Salicylic acid is a plant growth regulator that is used to tackle these types of salt and drought stress [15]. Salicylic acid can tolerate water and salt stress and enhances various functional processes such as photosynthesis, transpiration, and nutrient application. It is understood that SA can respond to these stresses [16]. It can alleviate both drought and salinity stress and improve water deficit stress tolerance in certain crop species, particularly cereals. It improves growth characteristics in water deficit stress-stressed conditions [17, 18].
Salicylic acid helps increase stress tolerance mechanisms in plants, especially in quinoa [19]. The SA is a growth regulator that supports the plant to withstand the deleterious impacts of drought stress. The SA is an inexpensive source that is used to promote development and production in quinoa plants having abiotic stress like scarcity of water, salinity, etc. This growth regulator together with silicon works best to alleviate these types of stresses [20]. Salicylic acid provides tolerance to deficit stress in quinoa because SA is famous for its capability to encourage a variety of metabolic responses in plants. It has been reported that the application of plant hormones is beneficial for promoting growth and yield [21]. A foliar spray of salicylic acid decreases the deficit water impacts on crops and maintains the yield [16].
Quinoa, known as Chenopodium quinoa, is an auspicious halophyte. It is a pseudo-cereal crop that contains high nutritional contents and high resistance against environmental stresses such as salinity, water deficit stress, etc. [22]. It is a member of the Amaranthaceae family derived from Latin America that can tolerate severe climatic alteration patterns. Seeds of quinoa have highly nutritious characteristics [23]. Quinoa is a dicot plant, and its tallness is 1.5-6.5 ft. Its cropping season is from 15 Oct-30 March. The temperature range for this crop to grow is 12-20ºC and its pH is equal to 8. It is cultivated in northern areas of Pakistan like Hunza and small plain areas like Bahawalpur. Quinoa leaves are broad, and these generate edible seeds and leaves [8]. The protein content in quinoa is about 12.5-16.7% and the fat content is about 5.5-8.5% [24].
Quinoa yield is about 2.5 tonnes per hectare in Pakistan. A single spikelet yields 200 g of quinoa grain [25]. It contains 71% water, 21% carbohydrate (Starch form), 4.4% protein, and 1.6% unsaturated fatty acids [26]. Grains of quinoa are rich in omega-3 and omega-6 fatty acids. Quinoa has 120 color varieties but red, black, and white are mostly used [27]. Quinoa is a cereal crop, and it can withstand harsh climatic stress conditions. It can tolerate the worst temperatures and lower temperatures such as from -40ºC to 350ºC. Quinoa is grown in sandy to loamy sand-type soil [28]. It is a C3 halophytic type plant. It is rich in protein content and amino acids.
The present research was primarily based on the theory that Si and SA can be utilized to reduce the adverse impacts of water shortage conditions on quinoa, thus increasing its production. By reducing the negative impacts of water shortage conditions in quinoa using Si and SA treatment, the current work filled the research gap. Researchers have done experiments for determining Si and SA impacts in reducing water deficit stress in other crops but their interactive effect in quinoa is not widely studied. Furthermore, work on comparative studies to evaluate the effectiveness of silicon and salicylic acid for reducing water deficit stress in quinoa is scarce. Based on this discussion, the present study was conducted to determine the impact of the combined application of silicon and salicylic acid for improving quinoa production, grain output, and development under water shortage stress.
Experimental Procedures
Experiment Setup
A pot experiment was carried out in the wirehouse of ISES, UAF. Each container was filled using 0.7 kg of soil and two water levels (100 and 60% FC) were maintained in pots by using a weighing method to develop water deficit conditions in the soil. Quinoa (Chenopodium quinoa) variety “V-17” was used. The suggested dose of NPK fertilizers for quinoa (i.e., 75-50-50 kg ha-1) was applied to all treatments before sowing. Irrigation was done in measured quantity to the pots according to the moisture condition of the soil. Three levels of silicon i.e., control, 100 and 200 mg kg-1 using potassium silicate as a source were used. Salicylic acid (1 mM) was foliar applied at the vegetative stage. Three foliar sprays with an interval of 10 days were done. There were thirty-six pots arranged in a completely randomized design (CDR) with factorial arrangements comprising 12 treatments in triplicate.
Measurement of Physiological Parameters
At the end of the vegetative stage, physical parameters such as chlorophyll (SPAD Value), relative water (RWC), and membrane stability (MSI) were investigated. Total chlorophyll contents (SPAD Value) in quinoa leaves was measured at the completion vegetative growth stage by the Soil Plant Analysis Development meter 502, which works on the light emission and transmission principle. For the determination of chlorophyll contents, three mature leaves of the quinoa plant were selected and placed under the SPAD meter. The average SPAD measurement of the leaf was determined [29]. Relative water content (RWC) was measured after the vegetative stage. For the measurement of RWC young leaves from the plant were taken and measured, following the procedure given by Barrs and Weatherly [30]. To calculate MSI, the method used was given by Sairam et al. [31].
Measurement of Growth Parameters
Crop was harvested as it reached maturation. Crop growth responses such as fresh and dry weight of shoot and root, plant height, and length of root were determined at the time of harvesting. Initially, samples were air-dried and then oven-dried for 72 h to determine shoot and root dry weight.
Measurement of Yield Parameters
Crop yield responses such as panicle length and grain yield were determined. Panicle length was calculated at harvesting time while grain yield was determined after oven-dried samples.
Determination of Na+ and K+ in the Shoot
For the determination of Na+ and K+ in shoot wet digestion was required which was done according to the method of Gargari et al. [32]. Na+ and K+ concentration was evaluated by using a Sherwood-410 flame photometer [33].
Statistical Analysis
Statistix 8.1 software was used to statistically examine data. The overall significance of data was assessed using the analysis of variance (ANOVA) method, and LSD was applied to compare the results at a 5% level of significance. All the analyses of various parameters were conducted using three replicates. The p-value<0.05 shows that there were significant differences among treatments [34].
Results
Physical Responses
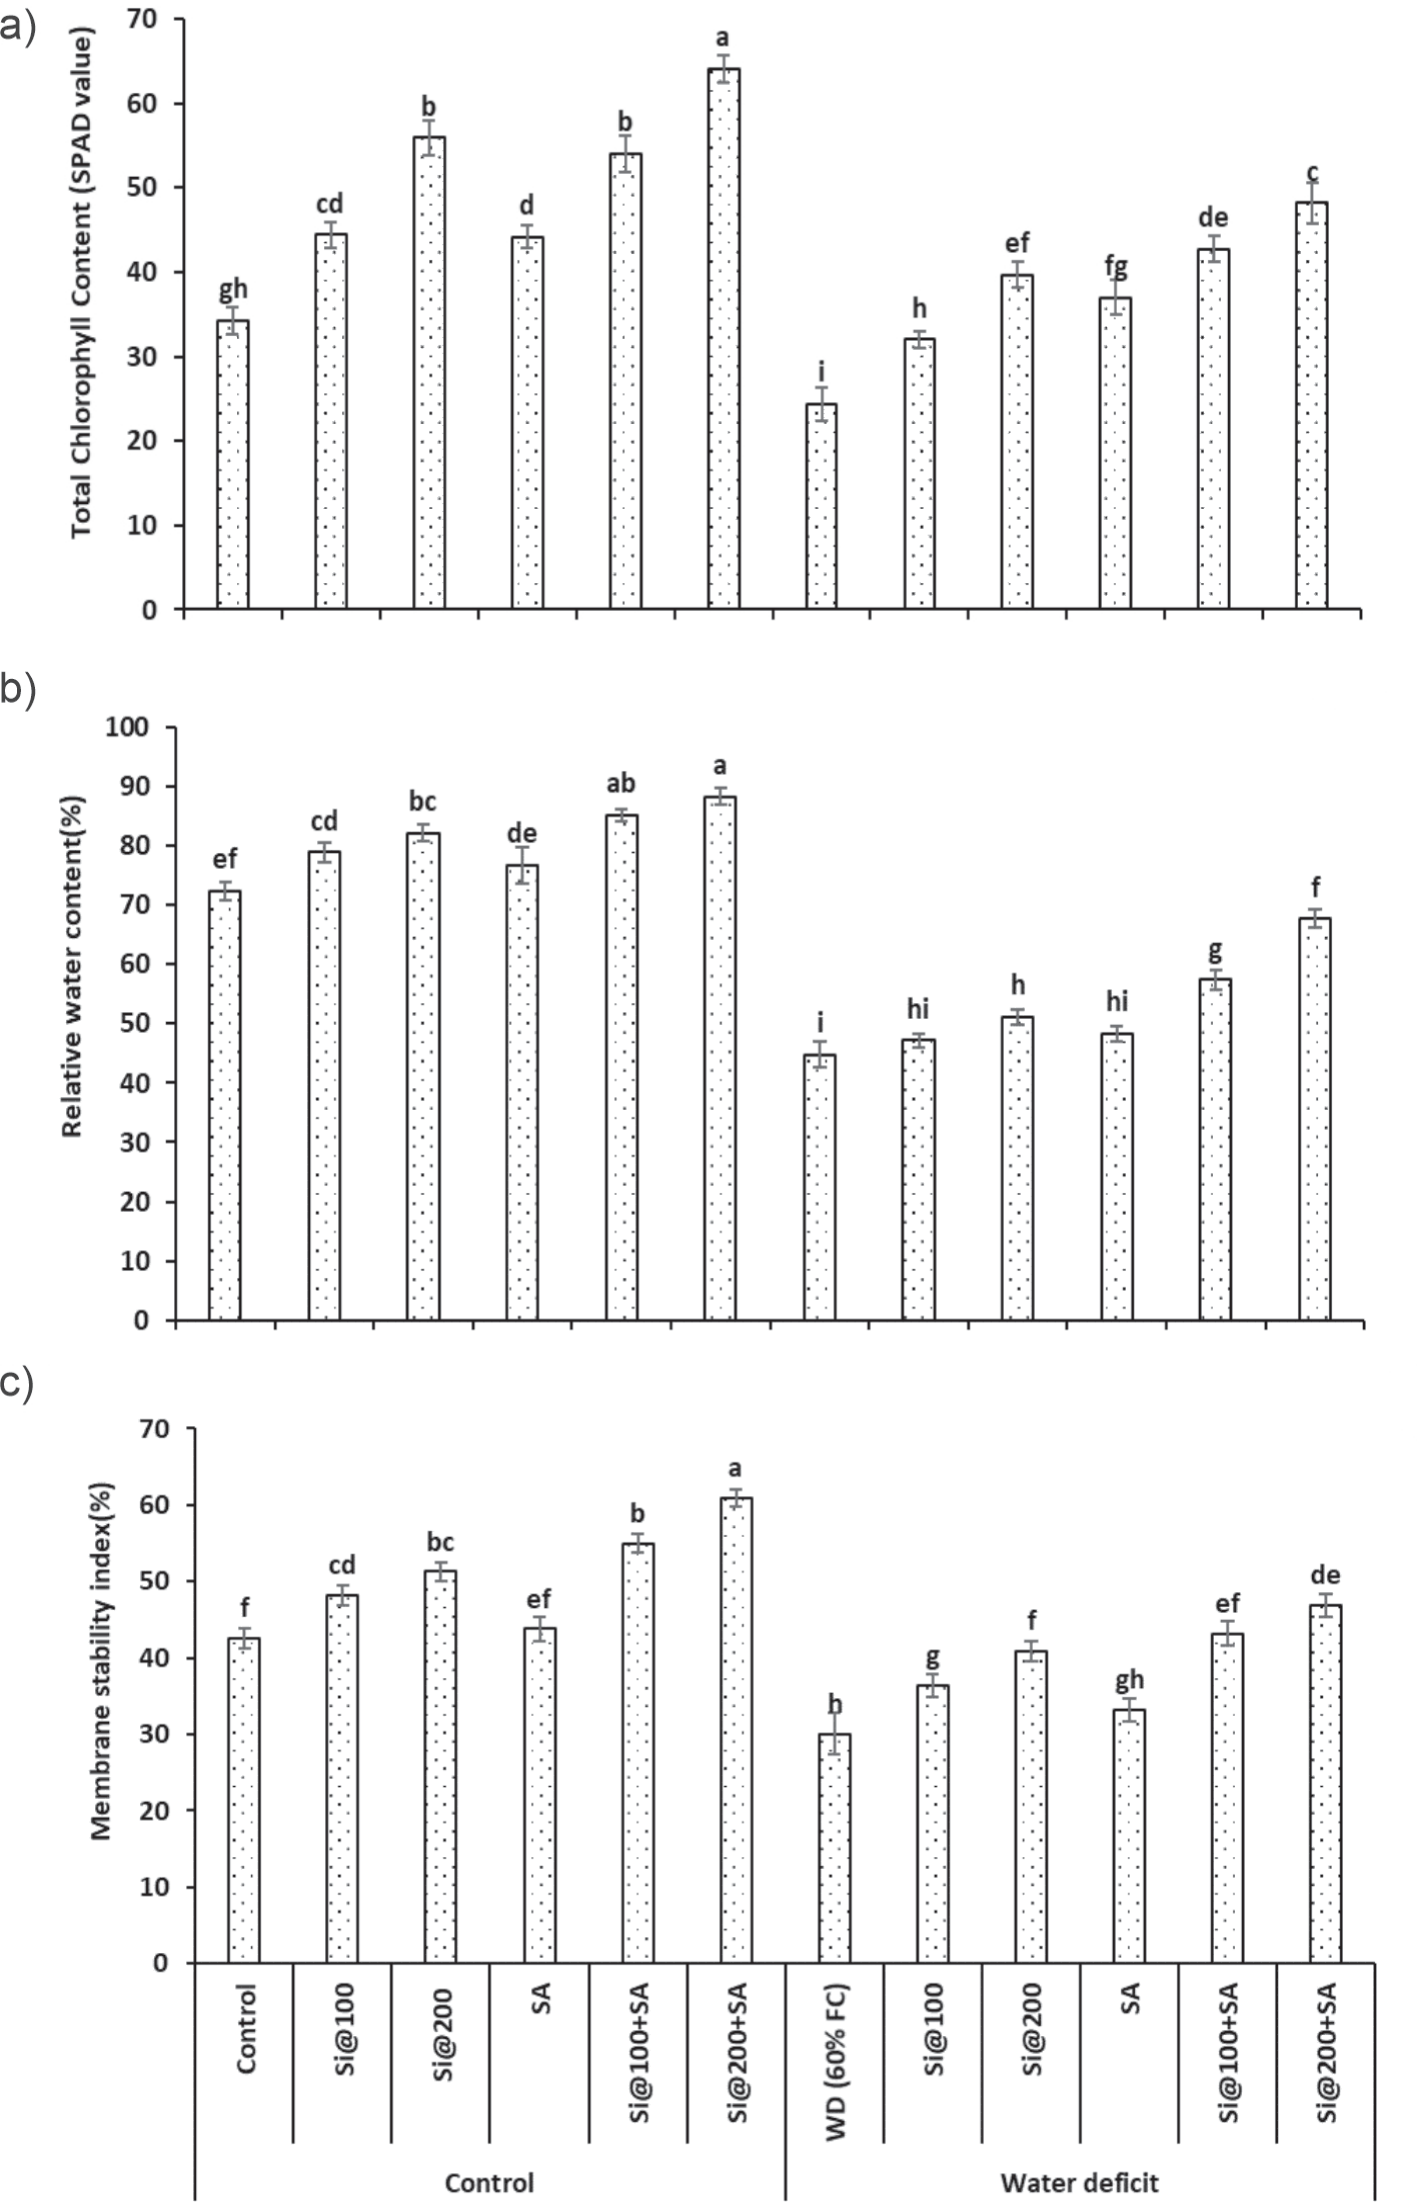
Physiological parameters of plants like chlorophyll content (Fig. 1a), relative water content (Fig. 1b), and membrane stability index (Fig. 1c) were affected significantly (p≤0.05) due to deficit water stress, applied treatments, and their interactive effect. As deficit water stress increases, TCC, RWC, and MSI decrease. Water deficit stress decreases TCC, RWC, and MSI by 29.02, 38.1, and 29.2% respectively as compared to the respective control when no amendment was applied. TCC, RWC, and MSI were enhanced due to applied silicon and salicylic acid in both normal and stress conditions. At moderate deficit water stress (60% FC), Si 100 mg kg-1, Si 200 mg kg-1, and SA 1 mM foliar spray enhanced TCC by 31.5, 63.1, and 51.9%, RWC by 5.35, 14.06, and 7.81%, and MSI by 21.2, 35.8 and 10.5% in comparison to respective controls. However, the combined dosage of Si 200 mg kg-1 with SA enhanced SPAD value (TCC) by 98.1%, RWC by 51.1%, and MSI by 55.9% respectively as compared to control in water deficit condition. Silicon treatment 200 mg kg-1 with 1 mM SA proved significantly efficient for alleviating deleterious effects of water deficiency stress on quinoa plant physical characteristics.
Fig. 1.
Chenopodium quinoa physiological parameters: a = TCC (SPAD value), b = RWC%, c = MSI% affected due to silicon and salicylic acid treatment in deficit water stress (Means + Standard error, n = 3). [LSD value for Si*SA interactions: TCC, Water deficit × trt = 3.9220; relative water content, Water deficit × trt = 5.0520; membrane stability index, Water deficit × trt = 4.1379].
Growth Responses
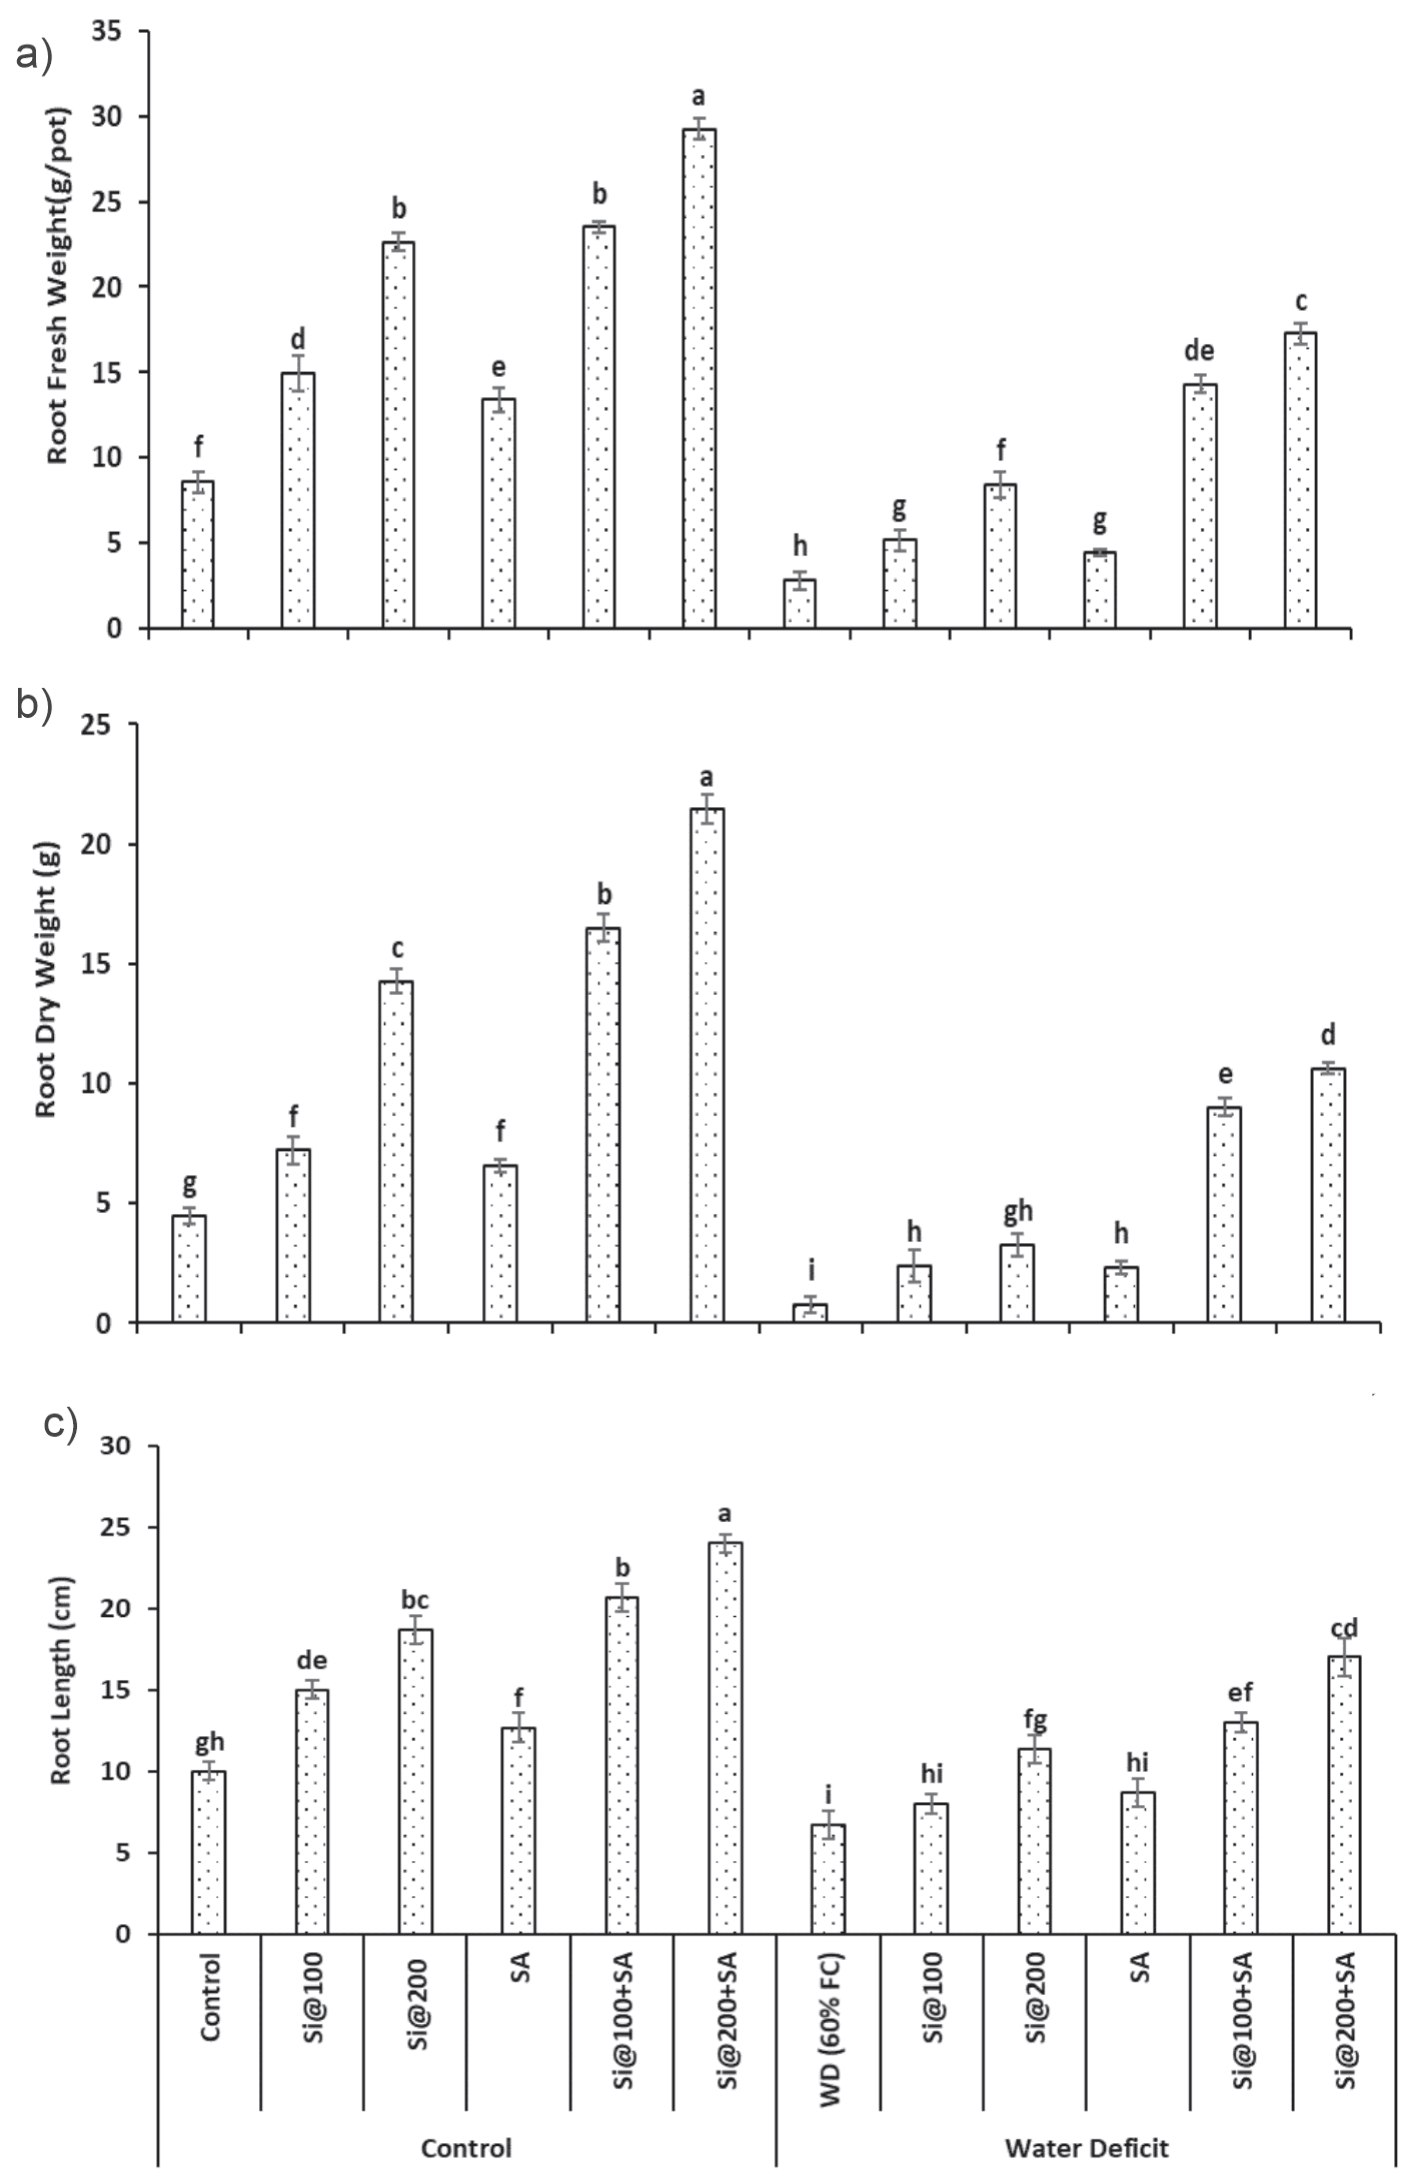
Growth parameters including height of the plant (Fig 2a), fresh and dry weights of the shoot (Fig 2b and 2c), fresh and dry weights of root (Fig 3a and 3b), and length of root (Fig. 3c) were affected substantially (p≤0.05) due to deficit water stress, applied treatments and its combined application impact. Water deficit stress decreases plant height by 46.05%, shoot fresh and dry weight by 62.5 and 70.6%, root fresh and dry weight by 67.09 and 82.2%, and root length by 33.3% respectively as compared to control. At moderate water deficit conditions (60% FC), application of Si 100 mg kg-1, Si 200 mg kg-1, and SA 1 mM enhanced plant height (26.8, 41.4 and 7.3%), shoot fresh (47.4, 86.0 and 52.9%) and dry (56.5, 143.4 and 52.1%) weight, root length (19.9, 69.8 and 29.9%), root fresh (83.7, 196.8 and 57.9%) and dry (200.0, 312.5 and 187.5%) weight respectively. However, combined application of Si 200 mg kg-1 with SA enhanced plant height by 87.8%, shoot fresh and dry weight by 143.3 and 195.1%, root fresh and dry weight by 510.2 and 1225.1%, and root length by 154.87% respectively as compared to respective control in water deficit condition. Silicon treatment 200 mg kg-1 with 1 mM SA proved significantly efficient for alleviating the deleterious effects of deficit water on quinoa growth parameters.
Fig. 2.
Chenopodium quinoa growth parameters a = plant height, b = fresh weight of shoot, c = dry weight of shoot impacted due to silicon and salicylic acid in deficit water stress (Means + Standard error, n = 3). [LSD value for Si*SA interactions: plant height, Water deficit × trt = 5.3201; shoot fresh weight, Water deficit × trt = 4.4753; shoot dry weight, Water deficit × trt = 4.223].
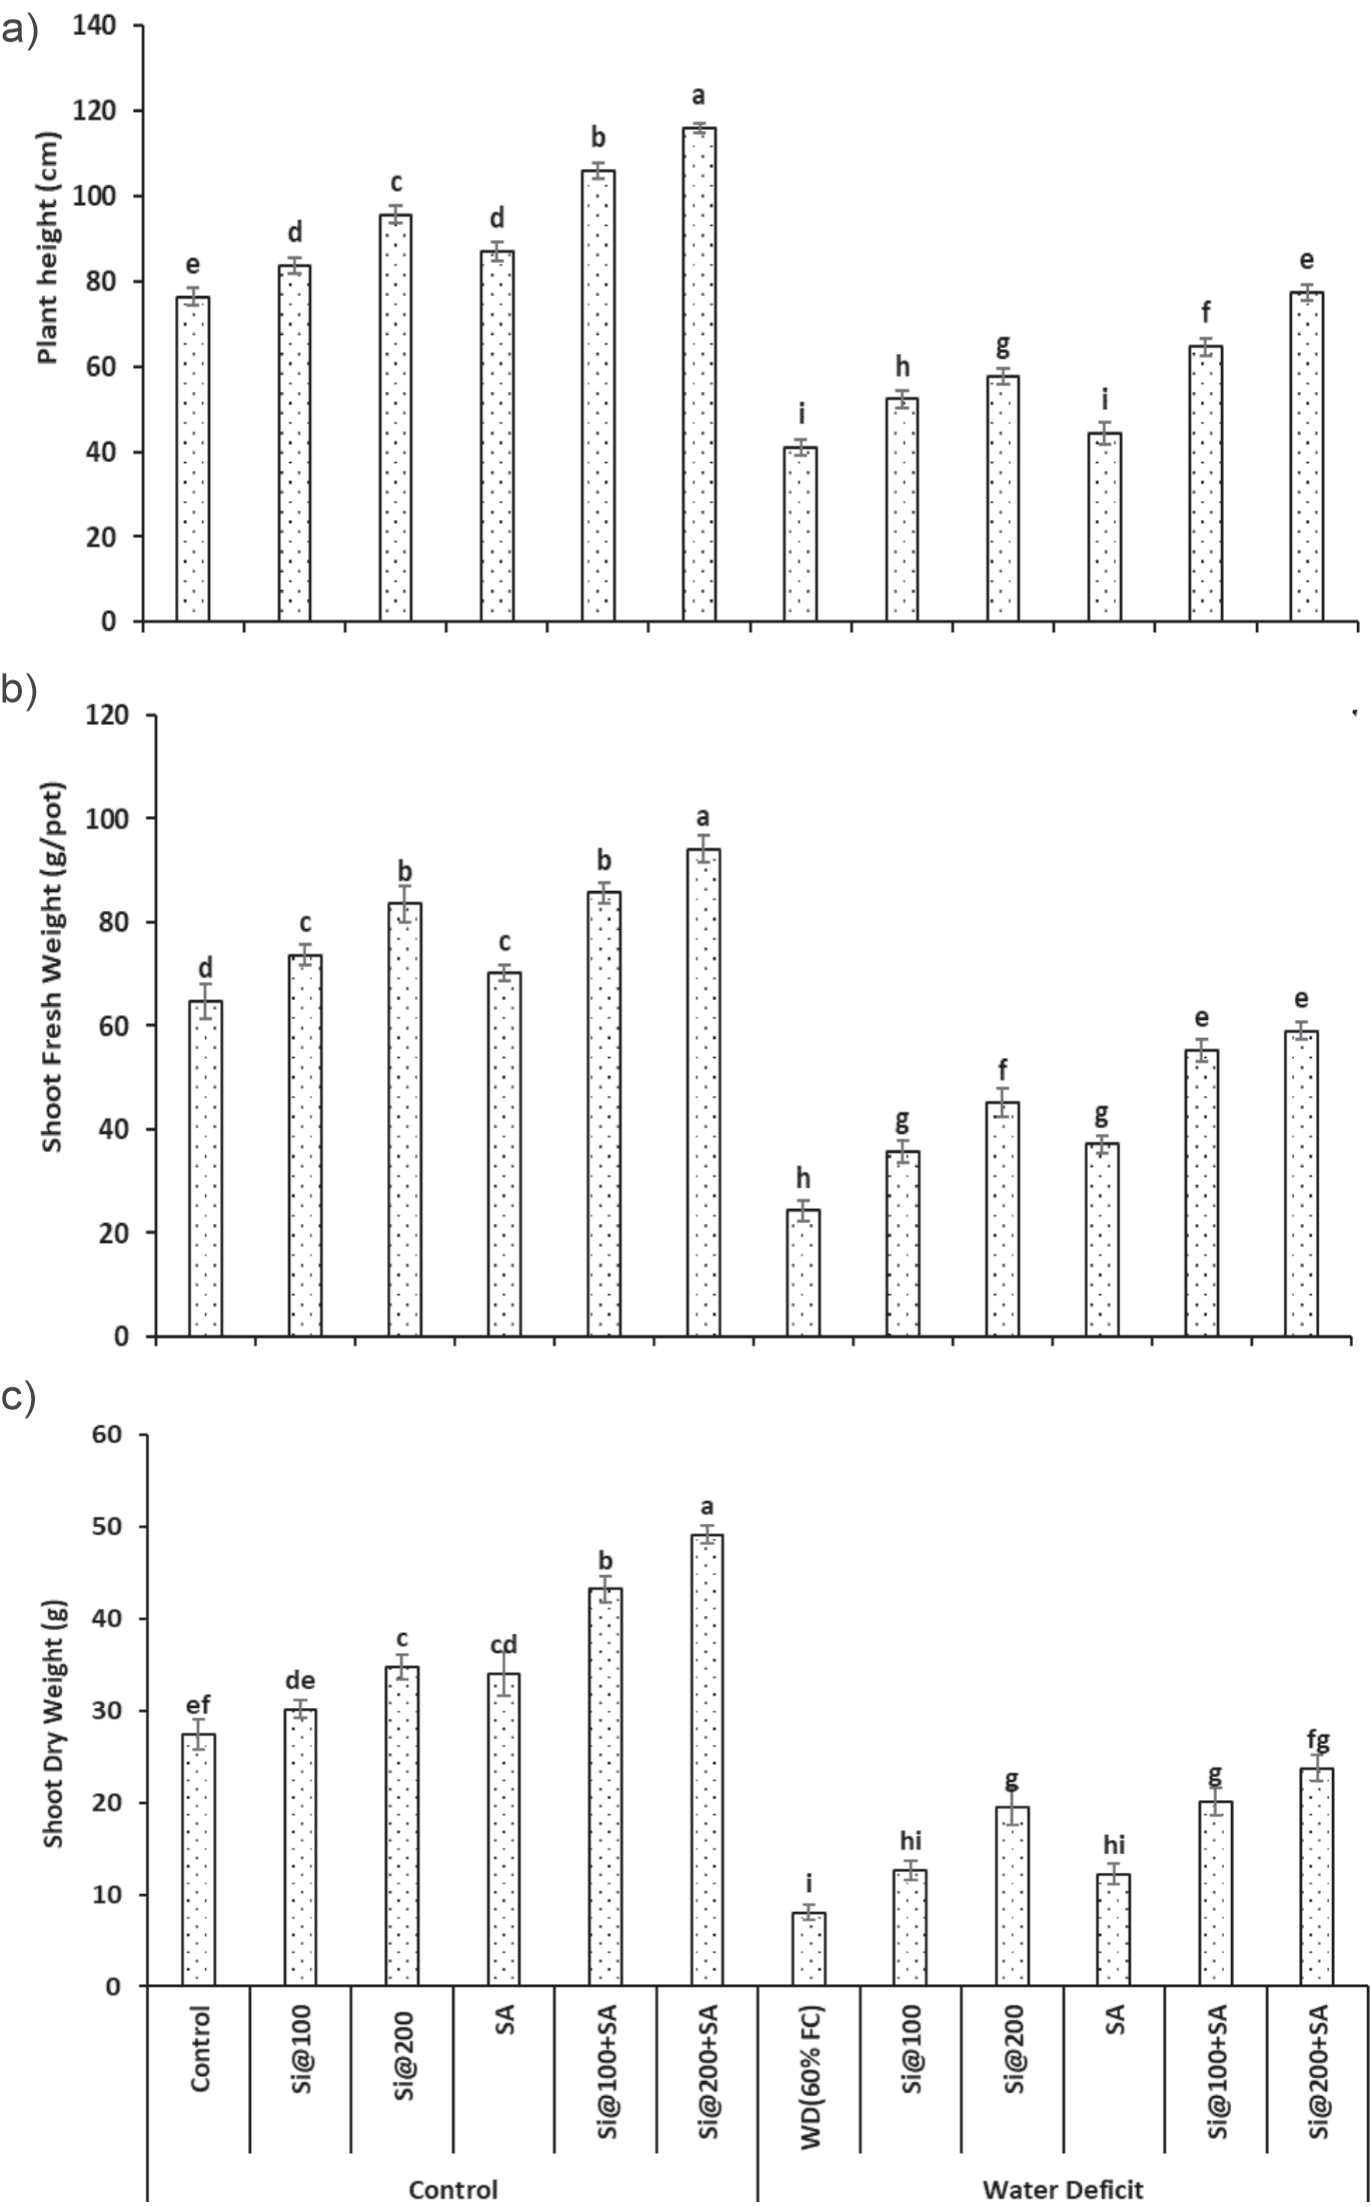
Fig. 3.
Chenopodium quinoa growth parameters a = fresh weight of root, b = dry weight of root, c = length of root impacted due to silicon and salicylic acid application in deficit water soil (Means + Standard error, n = 3). [LSD value for Si*SA interactions: fresh weight of root, Water deficit × trt = 1.4368; root dry weight, Water deficit × trt = 1.3070; root length, Water deficit × trt = 2.3101].
Yield Responses
Yield parameters including grain yield (Fig. 4a), and length of panicle (Fig. 4b) were influenced significantly (p≤0.05) due to deficit water condition, applied treatments, and their interactive impact. Water deficit stress decreases grain yield and panicle length by 70.5 and 49.9% in comparison to the respective control with no Si and SA applied. In deficit stress (60% FC), Si 100 mg kg-1, Si 200 mg kg-1, and foliar SA 1 mM enhanced grain yield by 159.01, 279.1 and 57.9%, and panicle length by 19.94, 69.86 and 32.98% respectively. However, the combined application of Silicon 200 mg kg-1 treatment with SA enhanced crop yield by 702.1% and panicle length by 124.8% as compared to respective control in deficit water conditions. Silicon treatment 200 mg kg-1 with 1 mM salicylic acid proved significantly efficient for alleviating the harmful effects of deficit water on quinoa yield responses.
Ionic Responses
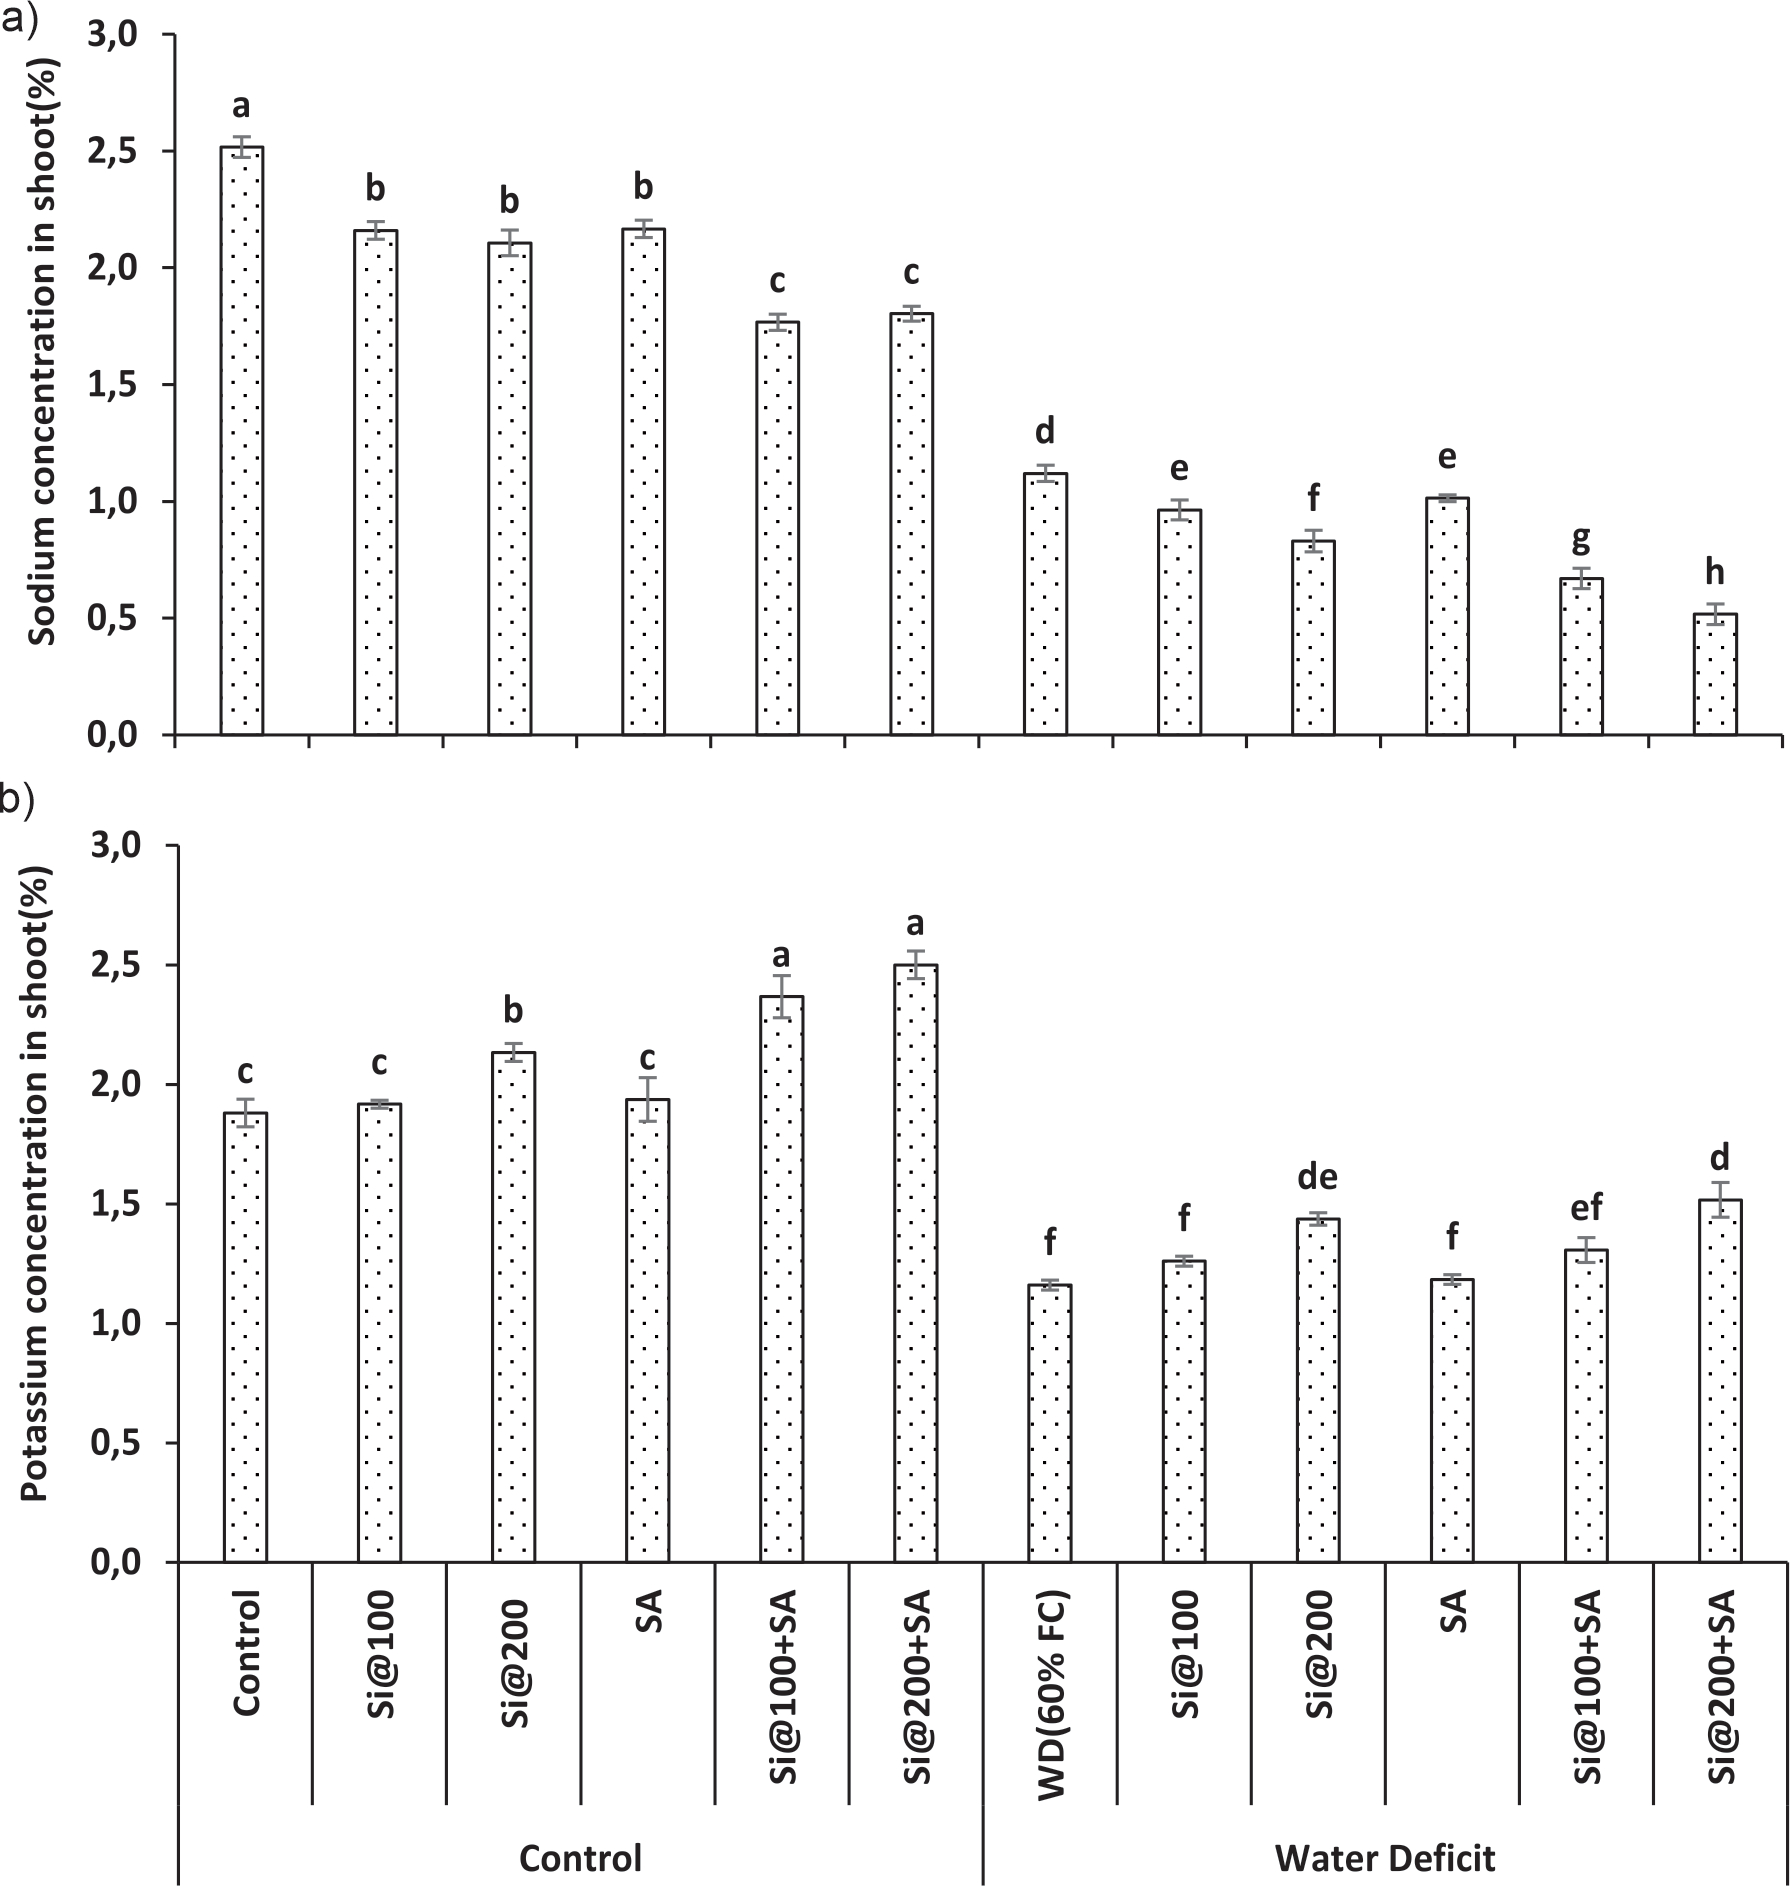
Ionic parameters include sodium concentration (Fig 5a) and potassium concentration (Fig 5b) in shoots that are significantly impacted (p≤0.05) due to water deficit conditions, applied treatments, and their interactive impact. Water deficit stress decreases Na+ and K+ concentration in the shoot by 55.2 and 38.2% in comparison to the respective control. Deficit water stress decreased Na+ and K+ concentration in the shoot but due to Si 100 mg kg-1, Si 200 mg kg-1 and SA 1 mM soil Na+ concentration remained decreased by 14.2, 25.8 and 9.8% while K+ concentration enhanced by 8.6, 24.1 and 62.0% in comparison with respective control. However, combined treatment of Si 200 mg kg-1 silicon with SA reduced Na+ concentration by 53.5% and increased K+ concentration by 31.0% as compared to respective control in water stress conditions. Silicon 200 mg kg-1 with 1 mM salicylic acid proved effective in decreasing the harmful effects on quinoa ionic responses.
Fig. 4.
Chenopodium quinoa yield parameters a = grain yield, b = panicle length impacted due to silicon and salicylic acid in deficit water stress (Means + Standard error, n = 3). [LSD value for Si*SA interactions: grain yield, Water deficit × trt = 1.5928; panicle length, Water deficit × trt = 2.2912].
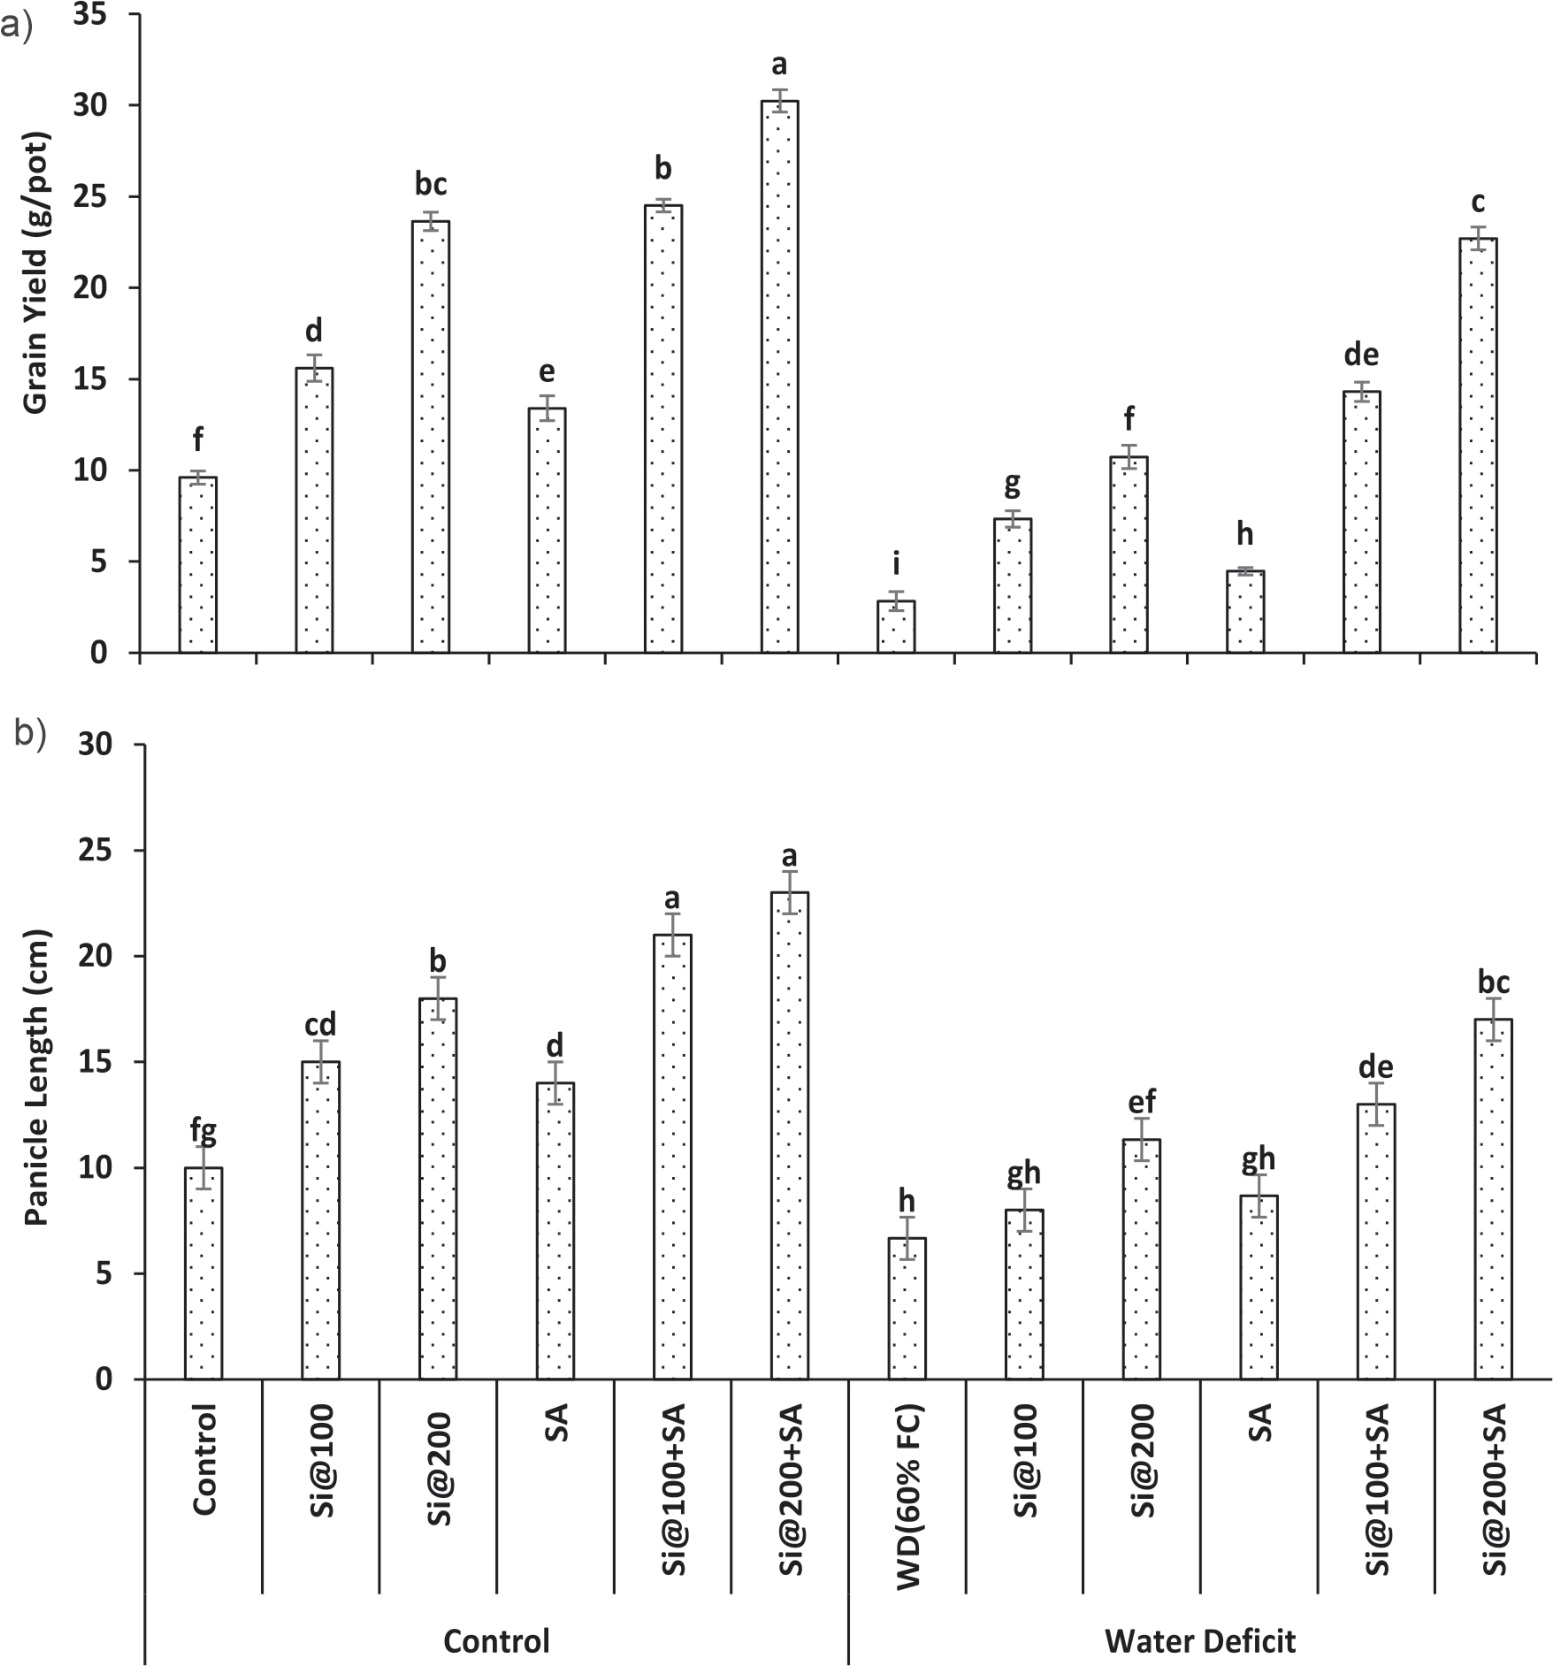
Fig. 5.
Chenopodium quinoa ionic parameters a = sodium concentration in shoot, b = potassium concentration in shoot influenced by Si and SA treatment in water deficit stress (Means + Standard error, n = 3). [LSD values for Si*SA interactions: sodium concentration in the shoot, Water deficit × trt = 0.1019; potassium concentration in the shoot, Water deficit × trt = 0.1630].
Discussion
Deficit water conditions reduce production, yield, and physiological, and biochemical characteristics in quinoa plants. Increasing levels of water deficit stress also increases the harmful effects of water deficit stress on quinoa. The current study results showed a significant reduction in grain yield, plant biomass, transpiration rate, green pigments, size and numbers of stomata, activity of photosynthesis, etc. Increased levels of certain osmolytes and decreased water stress are the results of development due to the application of silicon and salicylic acid [35]. These changes have resulted in improved leaf chlorophyll content, MSI, RWC, plant biomass, and grain yield under water deficit stress.
In the current study, water deficit stress significantly reduced the chlorophyll contents in quinoa. Previous studies showed that an excessive ROS (Reactive Oxygen Species) buildup inhibits photosynthetic activity and accelerates chlorophyll breakdown [36]. Silicon may stop the deterioration of chlorophyll due to lowering ROS regeneration and activating antioxidant enzymes. Salicylic acid is a growth regulator and reduces deleterious impacts caused by deficit water conditions on photosynthetic activity [37]. Potassium silicate is thought to be a source of K+ and Si components that are essential for maintaining and strengthening a plant’s photosynthetic system [38]. The SPAD value showed a significant impact due to deficit water conditions and applied treatments. In addition to boosting ATPase, DNA, and RNA production and maintaining the iconic equilibrium in leaves with water stress conditions, potassium silicate, and salicylic acid modulated stomatal conductance [39]. It has also been reported that as the availability of water decreases in plants to compensate for water deficiency plants close their stomata. As Si application in Lycopersicum esculentum improves water uptake and provides plants which results in stomatal increase in photosynthesis. As the stomata remain close the stomatal conductivity decreases, which results in a decrease in the photosynthetic rate [40]. The chlorophyll contents of water-deficit plants were recovered with the addition of both Si and SA together [41]. SPAD value (chlorophyll contents) was greatly improved by foliar SA and Si amendments, indicating that the combined application of Si and SA mitigates the harmful impacts caused by deficit water in quinoa.
Water deficit adversely affects the soil osmotic potential and ionic imbalance that ultimately reduces the availability of water to plants thus decreasing the RWC. According to our findings, RWC was decreased with increased water-scarce conditions. The same findings have been described by Soheili Movahhed et al. [42] who stated that RWC was considerably declined as the deficiency of water rose. Underwater stress conditions, deficiency of water in plants occurs as the evapotranspiration rate of plants becomes higher than its water uptake, accompanied by reduced relative water content which increases the leaf and root ratio and decreases the growth of plants [43]. When compared to the control plants, several of the silicon-treated plants demonstrated an increase in relative water content [44]. In water-deficient conditions, foliar application of SA and Si amendment has a more significant ameliorative effect on quinoa plants. The highest RWC was observed when silicon and salicylic acid combined amendment was applied during control conditions. As a physiological consequence of cellular moisture stress, the RWC is a suitable measurement of plant water status whereas plant moisture transport in the soil-plant-atmosphere continuum is assessed by water potential in corn [45].
According to our findings, MSI was significantly decreased in the pots treated with water deficit (60% FC). A higher concentration of ROS decreases the MSI and enhances the escaping of cell components [46]. As water stress increases, the availability of water for plant uptake decreases. Water is an important constituent of photosynthesis. Water uptake is also responsible for the uptake of nutrients absorbed in it by mass flow. Water also plays a role in enzyme activation, and stomata opening and closing. Our results are in line with the findings of Shahid and Thushar [47] observed a significant decrease in MSI of quinoa plants under water deficit stress. Si and SA both improve MSI in quinoa plants due to their chemical composition under deficit water stress [48]. Water stress also reduces specific ion toxicity i.e., Sodium [49]. According to Abdalla [50], Si has different mechanisms in plants against water stress like increasing antioxidant enzyme activity, making a defensive barrier in plants, and increasing oxidative stress. The combined application of both amendments (silicon and salicylic acid) showed positive results and recovered the plants from stress.
Water deficit stress reduces plant growth by inhibiting cell division and expansion and disrupting physiological and biochemical processes [51]. Silicon is deposited throughout the entire organism when the roots absorb Si from the soil and carry it to the shoot region via a transpiration stream [52]. There was a significant effect of water deficit, applied treatments, and their interaction on the length, fresh, and dry weight of root and shoot of quinoa plants. Water stress decreased plant biomass significantly. Under deficit water conditions, there is a decrease in the roots and shoots of the plant in stressed conditions [53]. Silicon and salicylic acid application has been recognized as it enhanced the dry weight of roots and shoots under water deficit stress conditions [54]. Plant hormones, SA which are generated by certain organs and control a variety of growth and developmental processes, can be stimulated by the accumulated Si [55, 56].
Our findings of the present study are consistent with Elgharably [57] who stated a substantial decline in the accumulation of total dry mass, straw, and yield of wheat plants by increasing the water deficit during the growing season. The combined application of SA and Si significantly lessened the negative effects of water stress on quinoa, by increasing Si uptake to leaf tissues, maintaining essential nutrient flow from roots to plant leaves, and maintaining water holding capacity. The improved assimilate translocation and biosynthesis as well as osmoregulation protected leaf tissues from water deficit-induced oxidative stress [58].
According to our results shoot growth was significantly reduced under moderate water deficit stress (60% FC). Amini et al. [59] also reported that water scarcity adversely affects various physiological and biochemical processes in plants that ultimately reduce shoot growth. Sabagh et al. [60] have reported that water deficiency in plants causes osmotic stress, nutrient imbalance, and specific ion effect which ultimately reduces the availability of water, nutrients, and photosynthetic activity due to which shoot growth also decreases. Water deficit stress has adverse effects on shoot development because water and nutrients are deficient. Fathalla and El-Mageed [61] also reported that under deficit water stress conditions due to less availability of water and nutrients, shoot growth significantly decreased. The same findings have also been reported by Abbas et al. [62] and Benjamin et al. [63] who stated that water deficit significantly decreased the shoot growth of eggplant. The osmotic effect reduces the activity of meristematic cells in the shoot axis thereby cell elongation and consequently plant height of maize [64]. Application of Si and SA was proved to be effective in increasing shoot growth of quinoa even in stress conditions. Their interactive effect showed better results of shoot growth (shoot length, dry and fresh weights) both in water stress and control conditions.
According to Jangpromma et al. [65], corn’s root development is reduced as the amount of water deficiency stress rises. The results obtained by Boutraa et al. [66] also showed a reduction in root growth with increasing levels of water stress in wheat. Reduction in root growth in water-deficit soil was also reported by Munns [67] and Saidi et al. [68] also stated that due to deficit water conditions; the development of roots also declined. Auxin is a crucial root development regulator in several crops, including tomatoes and maize [68, 69]. According to the findings of this study, quinoa showed decreased root development in deficit water stress.
Water deficit stress had adverse effects on grain yield. Water stress reduces the availability of nutrients that ultimately reduce grain weight [70]. Results obtained by Sabagh et al. [60] are in line with our findings. They reported that grain weight was significantly reduced due to deficit water stress. The reduction in grain weight with an increase in water deficit stress was also reported by Dietz et al. [71], Fathalla and El-Mageed [61], and Alqudah et al. [70]. Water deficiency has adverse effects on the grain yield of crops by decreasing nutrient availability. Sabagh et al. [60] also reported that under deficit water conditions due to less water and nutrient availability grain yield of wheat significantly decreased.
Similar results were also reported by Alqudah et al. [70] and Venuprasad et al. [72], who said that water deficit stress decreased the uptake of nutrients that ultimately reduced the grain yield. Si is a beneficial element used as an amendment with foliar SA to decrease the harmful effects of water deficit on plants due to its various mechanisms; nutrient uptake, increasing antioxidant enzyme activity, decreased Na+ toxicity, and enhanced K+ ion activity. Application of Si and SA was proved to be effective in increasing the grain yield of quinoa even in stress conditions. Their interactive effect showed better results of grain yield in water stress as well as control conditions.
Water deficit also affects the concentration of Na+ in the shoot. Due to the deficiency of water in plants, ionic parameters like Na+ and K+ concentrations are also reduced. The results of our study showed an increase in water deficit significantly decreased Na concentration in the shoot. Our results are also justified by the results of Ali and Rab [73] and da Silva et al. [74] who reported a decrease in Na+ concentration in shoots with an increase in water stress. The reduction in Na+ intake and aggregation in plants is one of the significant pathways of resistance for the plant to deficit water stress. It has been stated generally that the use of Si and foliar SA treatment in quinoa plants under the stress of water deficit minimized the uptake of Na+ reduced the Na+ ratio and improved the K+ ratio [73-76]. Silicon application reduced water shortage both in the roots and shoots of the Abelmoschus esculentus plant under deficit water stress [75]. Similarly, the use of Si in grapevine roots (Vitis vinifera L.) has declined the deleterious effects of deficit water stress in plants [77]. Na+ concentration is reduced in the roots of maize and wheat plants [76, 77]. Na+ concentration in the shoot significantly decreased due to water stress. Our research showed that Si and SA combined application can alter the deleterious effects of moderate water deficit stress (60% FC) in quinoa. Application of Si and SA was proved to be effective in decreasing Na+ conc. of quinoa in stress conditions. Their interactive effect showed better results and decreased Na+ conc. in both stress and control conditions. Si and SA both reduced sodium concentration in the shoot under water deficit conditions.
Water deficit stress drastically affects the K+ concentration in shoots as well. Deficit water stress significantly decreased ion conc. like K+ ions in the shoot. The results of our study showed an increase in water deficit significantly decreased K+ concentration in the shoot. In most plants, it was observed that the addition of Si and SA enhanced the K translocation and absorption from root to shoot although absorption and movement of Na+ and Cr2+ decreased [78, 79]. In addition, the meditation of Si activated the H-ATPase’s function of the plasma membrane of the root, as recorded in aloe [80] and barley [81] due to the reduction in absorption of Na+.
Low availability of K+ to the plants reduced crop production in water stress situations while Si and SA application increased the K+ content of shoots and crop production [35], and enhanced the yield of the crop. From the above-described studies, it may be presumed with confidence that silicon and foliar salicylic acid interaction reduced the deleterious impacts caused due to deficit water conditions in quinoa, thereby boosting quinoa production and output in deficit water stress.
Conclusions
According to the current study, silicon and salicylic acid were applied to the quinoa crop to improve production and grain output and decrease deficit water stress. Crop production and yield have decreased due to water shortage stress. However, silicon with an external application of salicylic acid showed improvement in growth and yield parameters with the reduction of deficit water stress. Silicon 200 mg kg-1 and salicylic acid 1 mM foliar spray proved effective for increasing crop output and production under water deficit conditions. It is therefore concluded that by increasing water deficiency stress in quinoa, all indices were decreased dramatically. The interactive effect of Si and foliar SA certainly succeeded in reducing the water stress in the medium of growth. Findings revealed that the combined application of Si 200 mg kg-1 and SA 1 mM was found the most beneficial for reducing the harmful effects of deficit water conditions.

