

Introduction
Fig. 1.
Area of investigation on which sampling of phytoplankton communities was performed in the Bay area (BK1, BK2, BK3, and BK4) during 2019 (QGIS48) (http://www.qgis.org).
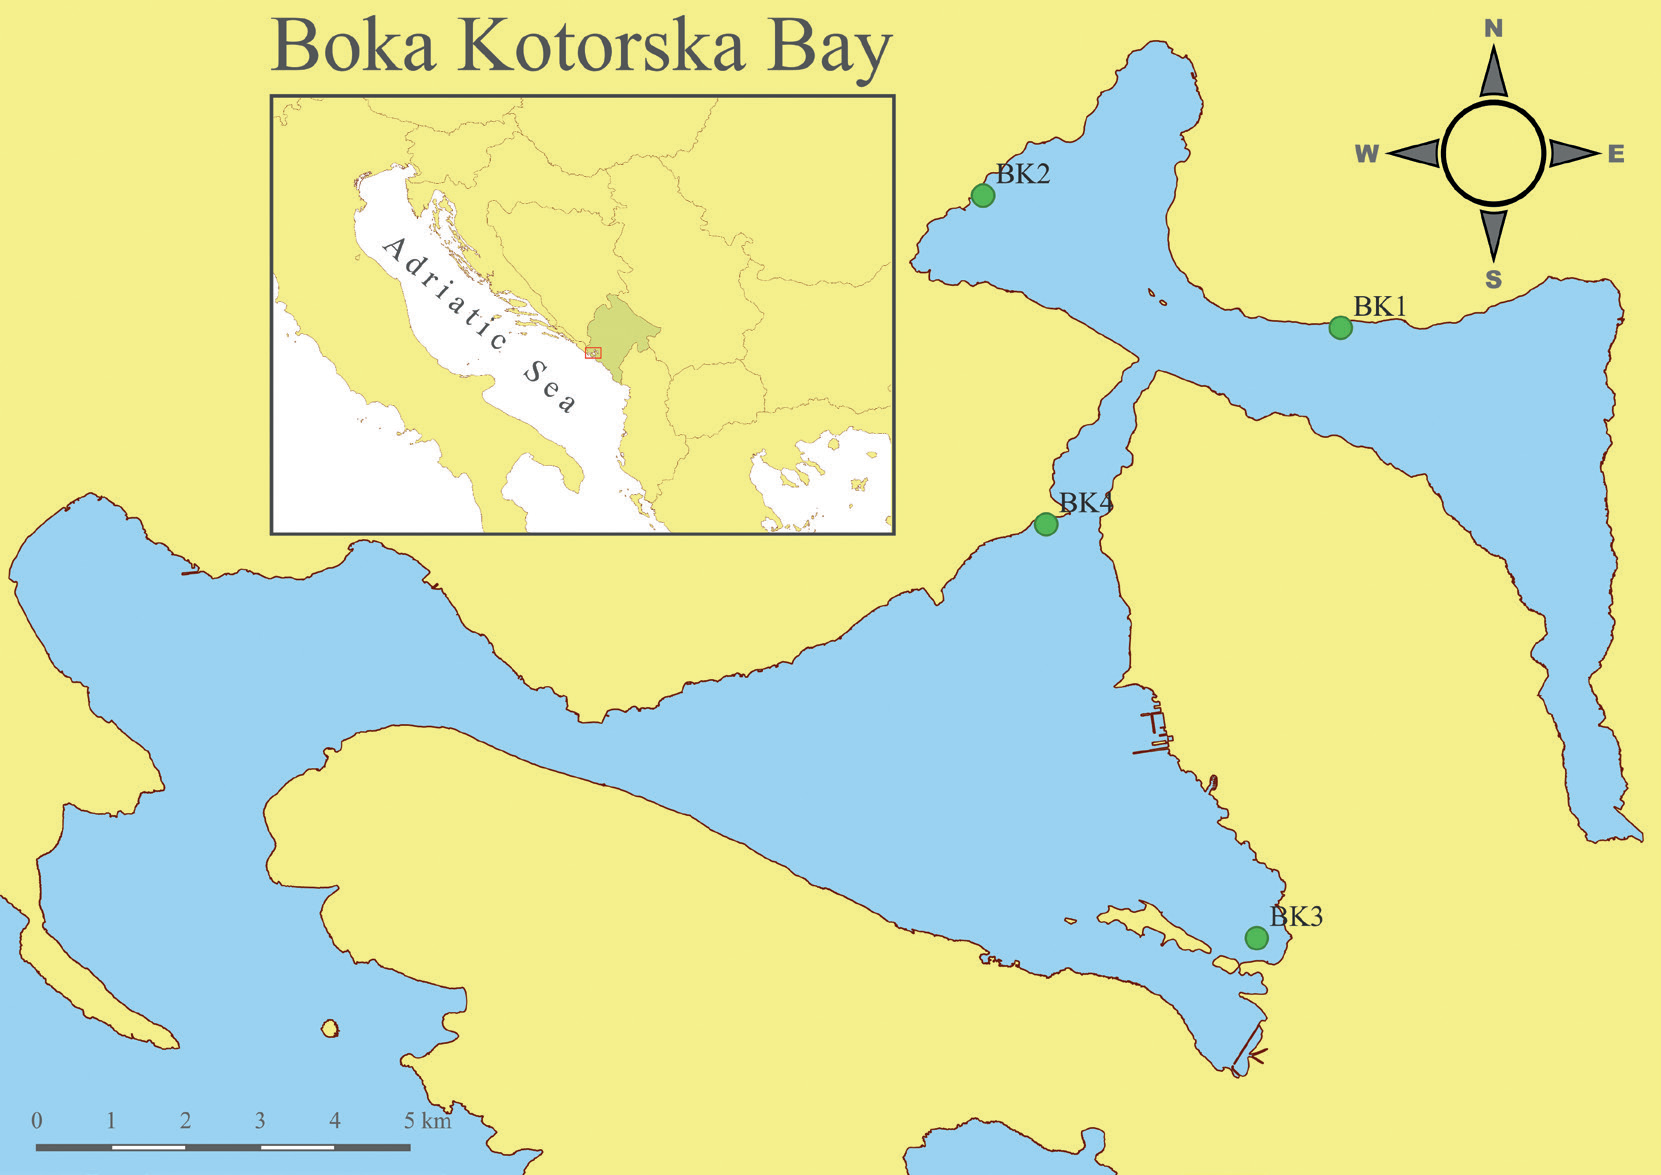
The Montenegrin coast comprises the semi-enclosed, fjord-like Boka Kotorska Bay, as well as the open coastal area of the sea. Boka Kotorska Bay is a relatively small transitional system that presents an environmental bound-ary between land and sea, with specific community as-semblages [1]. The area of Boka Kotorska Bay has higher precipitation due to the presence of high karstic mountain massifs [2]. Additionally, the bay area is under greater influence from the land compared to the open coastal region.
The species of the genus Ostreopsis are marine, benthic dinoflagellates. They primarily inhabit epiphytically on benthic macroalgae, although they can also be found on sand, rocks, and in the water column. The increased abundance of Ostreopsis species can lead to the formation of a brownish mucilaginous biofilm on various substrates.
Toxic species belonging to the marine dinoflagellate genus Ostreopsis are known to be present in various en-vironments, from tropical and sub-tropical to temperate areas [3]. Mass appearances of the toxic dinoflagellate genus Ostreopsis (≥10000 cells/l) have been noticed to cause dangerous respiratory problems in humans exposed to aerosols [4-6]. Additionally, Ostreopsis species produce different toxins that can be transferred to certain fish and invertebrates, posing a potential risk of food poisoning to humans as well [3, 7, 8]. Also Ostreopsis blooms have a negative impact, causing mass mortalities of certain invertebrates [3] caused either by oxygen limitation due to the excess of microalgal biomass or specific ecotoxic compounds.
In Croatian waters, the first record of Ostreopsis cf. ovata was reported from the central Adriatic Kaštela Bay in 1984 [9]. Available literature confirms that, in the Adriatic Sea, the highest abundances of Ostreopsis species were observed along the Marche and Apulia coasts [9, 10]. The highest abundances on macroalgae were noted in 2008 and 2009, while the highest abundances in seawater were reported in 2006, 2010, and 2016 (reaching values up to 107 cells/l) [9].
The scope of this paper is to inform about the first records of toxic species on the Montenegrin coast and to emphasize the necessity of monitoring the presence and abundance of these species, knowing the negative effects they have on marine ecosystems and human health.
Material and Methods
Study Area
Sampling for Ostreopsis analysis was carried out as part of the monthly monitoring program at four mussel farms in the area of Boka Kotorska Bay. It is important to note that only data from October 2023 are considered for both total phytoplankton and Ostreopsis analysis (see Fig. 1). Water samples for physico-chemical and phytoplankton analysis were taken from one depth, up to 5 meters (maximal depth at position Dražin vrt (BK1) where Ostreopsis was observed is 23.3 m, while on other investigated positions maximal depths were BK-2-24.5 m, BK3-21.9 m, and BK4-7.6 m). Samples were taken with 5 L Niskin bottles. Two parameters (temperature and salinity) were measured directly in situ using a multi-parameter portable device (Multiline P4; WTW).
Table 1.
Maximal (Max.), minimal (Min.), and average values of temperature (Tem.) and Salinity (Sal.) and maximal, minimal, and average abundances of total microplankton (TMP) and total nanoplankton (TNP) at investigation area during 2023.
| Max | Min | Avg | STD | |
|---|---|---|---|---|
| Tem. (°C) | 21.8 | 20.2 | 21.25 | 0.73 |
| Sal. (psu) | 37.2 | 35.2 | 36.05 | 0.83 |
| TMP (cells/l) | 8.96 × 10⁴ | 4.74 × 10⁴ | 6.98 × 10⁴ | 1.93 × 10⁴ |
| TNP (cells/l) | 1.35 × 10⁵ | 8.72 × 10⁴ | 1.08 × 10⁵ | 2.13 × 10⁵ |
For the sampling of phytoplankton, 5-L Niskin bottles were used, and the collected samples were transferred into 250 ml plastic bottles. Preservation of samples was performed using a 4% neutralized formalin solution. Samples were transported in a refrigerator under dark conditions at a temperature of approximately 8 ± 3°C. The sampling was performed according to the guidelines in MEST ISO 5667-9:2020-Water quality – Sampling Part 9: Guidance on sampling from marine waters.
Phytoplankton cells were counted using a Zeiss Axio inverted microscope (Axio Observer A1) in accordance with the method of Utermöhl (1958) [11] (MEST EN 15204: 2014-Water quality – Guidance standard on the enumeration of phytoplankton using inverted microscopy). In the laboratory, samples were settled in sedimentation chambers of 25 ml, and after a period of sedimentation of 24 h, we started with the processing of the determination. Enumeration was performed at the following magnifications: 200 ×, 400 ×, and 630 ×. The whole bottom chamber (taxa larger than 30 μm) was crossed at a magnification of 200 × (enumeration of Ostreopsis cells was done this way), while at the same magnification, two transects were used for counting abundant microplankton (> 20 μm). Small phytoplankton (nanophytoplankton 2–20 μm) were counted at magnifications of 400 × and 630 × using 10 randomly selected fields. Determination of phytoplankton species was performed using an appropriate key [12–15]. Non-identified microalgae were classified into taxonomic categories: nanoflagellates, small dinoflagellates, small coccolithophores, and chrysophytes.
Results and Discussions
Environmental Data
During the research period (October 2023), maximal temperature was recorded at position BK1-Dražin vrt and it was 21.8°C, while minimal temperature values were observed at position BK2-Lipci (20.2°C). During the summer period, temperature ranged from 24.1–25.0°C (Table 1). In the north Adriatic Sea, it was observed that the highest abundances of Ostreopsis do not match with the highest water temperature values in all areas.
Accoroni and Totti [16] suggested that environmental factors play a crucial role in Ostreopsis blooms, as the species tends to produce more toxins under suboptimal conditions. It is interesting that Ostreopsis cf. ovata can produce both temporary and resting cysts. Specifically, resting cysts have been noticed to germinate for up to 5 months after formation at 25°C, but not at 21°C. This temperature-dependent cyst germination suggests that temperature may be a key factor influencing the Ostreopsis cf. ovata blooms. This observation could explain the presence of Ostreopsis in our study during October, when temperatures were lower compared to the summer period.
In the northern Adriatic Sea, Ostreopsis blooms often occur approximately 30 days after temperatures reach 25°C, indicating that other factors besides temperature may also impact the growth of Ostreopsis cf. ovata [16]. Several authors have similarly emphasized the role of temperature in favoring Ostreopsis cf. ovata blooms [17].
Regarding values of salinity concentration, the highest salinity was measured (37.2 psu) in position BK3-Kalardovo, while the lowest value of salinity was in position BK1-Dražin vrt (35.2 psu) (Table 1).
Accoroni and Totti 2016; Pezzolesi et al. [16, 18] observed that benthic dinoflagellates growth is favored by lower salinity waters, and mostly occurs in periods of maximal rainfall, which was noticed in our study. During the study of the relationships between algal growth and salinity, other factors, such as levels of nutrients (which are typically associated with low salinity waters) have to be considered [16]. On the other side, some studies showed that Ostreopsis cf. ovata grew better under higher salinity conditions, but others suggested that it depends on strains [17]. A lot of studies have emphasized the influence of environmental factors on Ostreopsis blooms, yet the full complexity of conditions leading to these blooms remains incompletely understood [16]. Both abiotic and biotic factors play significant roles, including interactions with other organisms and the use of organic forms of nutrients. It is interesting that several harmful algal bloom (HAB) genera have been shown to need organic forms of nutrients to meet their nutritional requirements. Furthermore, the effects of biotic interactions on Ostreopsis should be considered. However, only a few studies have investigated these interactions, focusing on bacteria, diatoms, and macroalgae [16, 19].
In the south-eastern Mediterranean Sea [20], it was observed that between salinity of 25 psu and 35 psu, Ostreopsis cf. ovata cells were almost absent in the water column. Its growth is recorded, in the Gulf of Gabès at a salinity of 35 psu and reaching its peak at a salinity of 45 psu.
Phytoplankton Parameters
The abundance of total phytoplankton during October 2023, at position Dražin vrt in the area of the Boka Kotorska Bay reached values up to 105 cells/l. The highest recorded value of microplankton- higher phytoplankton fraction was at position Kalardovo BK3 (8.96 × 10⁴ cells/l), while the lowest abundance was at position Lipci-BK3 and it was 4.74 × 10⁴ cell/s. Nanoplankton – smaller fraction was the highest at position BK3-Kalardovo (1.35 × 10⁵ cells/l) and the lowest abundance was recorded at position Lipci-BK2 (8.72 × 10⁴ cells/l) (Table 1).
The distributions of total microplankton (TMP) and phytoplankton groups-diatoms and dinoflagellates along the research area were presented (Fig. 2). Diatoms were the dominant group of phytoplankton with maximum abundance at position BK3 (8.62 × 10⁴ cells/l).
Dinoflagellates were the second most frequent and abundant phytoplankton group during the research period. Previously, the dominance of diatoms was observed in both Boka Kotorska Bay [21, 22] and the northern Adriatic Sea [23, 24] on both sides.
Dinoflagellates values ranged up to 103 cells/l. The highest abundance of dinoflagellates was recorded at the position Dražin vrt (BK1) reaching 6.96 × 10³ cells/l, while the lowest abundance of dinoflagellates was recorded at the position Sveta Nedjelja (BK4), with 320 cells/l.
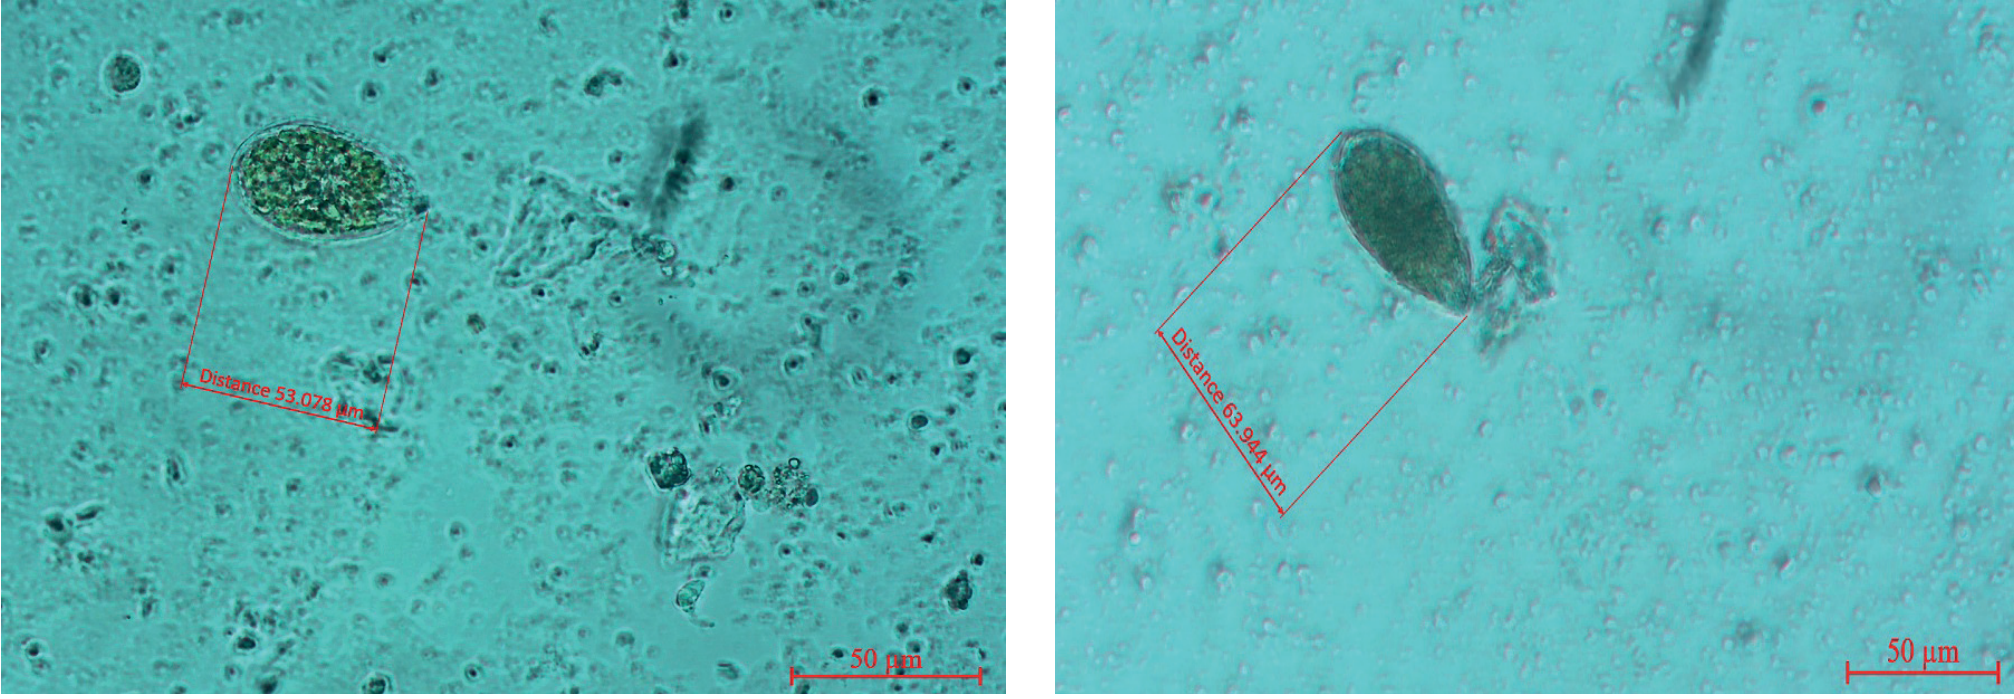
In the area of Boka Kotorska Bay and in the Montenegrin coast the presence of the species from the genus Ostreopsis was recorded for the first time. The species was recorded in the water column, up to a depth of 5 m (Fig. 3A, Fig. 3B). The abundance of the species was 5.92 × 10³ cells/l while the total abundance of dinoflagellates at position Dražin vrt was 6.96 × 10³ cells/l. This confirms that at position Dražin vrt (BK1) in the water mass species, Ostreopsis cf. ovata contributed mostly to dinoflagellates abundances.
The presence of Ostreopsis cf. ovata (with an abundance of 5.92 × 10³ cells/l in water) was recorded during the fall period in October 2023 as part of our regular monitoring. Additionally, during the research (October 2023) at BK1 position several other dinoflagellate species were recorded: Gonyaulax spp., Gyrodinium fusiforme, Prorocentrum com-pressum, P. triestinum, .Protoperidinium crassipes, Tripos kofoidii, and T. lineatus. On position BK2 it was noticed presence of dinoflagellate Dinophysis acuta and at BK3 position presence of Phalacroma rotundatum.
Kužat et al. [25] observed higher abundances of Ostreopsis in the north-eastern Adriatic coast (Istrian peninsula and Kvarner Bay) compared to the south-eastern Adriatic Sea (the area around the city of Dubrovnik) at the end of the summer period. This discrepancy with our findings may be due to unfavorable ecological conditions, which can change the timing of Ostreopsis presence or bloom events. In the study by Kužat et al. in 2021 [25], lower temperatures and salinity resulting from inputs of submersed coastal freshwater springs were found to influence the presence of Ostreopsis at some stations. These findings underscore the necessity for more detailed monitoring along the entire Adriatic coast (both north-eastern and south-eastern parts).
Furthermore, in the north-western Adriatic [6, 16], it was documented that the peak of Ostreopsis at some stations could occur earlier and with higher abundances due to changes in ecological conditions.
In their study, Kužat et al. [25] observed differences in ecological conditions, including anthropogenic influence and eutrophication, at all sampling stations where the presence and blooms of Ostreopsis cells were recorded. This confirms the notion that anthropogenic pressure increases the risk of harmful Ostreopsis cf. ovata blooms along the generally oligotrophic eastern Adriatic coast.
However, while significantly higher cell abundances corresponded to densely populated areas around the cities of Poreč and Rovinj, the direct influence of anthropogenic factors on the occurrence of Ostreopsis blooms is present. Although the correlation between higher abundances of Ostreopsis cf. ovata and the trophic load discharged into marine waters from anthropogenic sources has been noticed, a clear relationship between anthropogenic impact and Ostreopsis cf. ovata abundances has yet to be confirmed [16]. Nonetheless, in the northern Adriatic Sea, it was observed that during Ostreopsis blooms, concentrations of certain substances were higher than during the rest of the study period [17].
In temperate areas, as noted by Accorini and Totti [16], the growth of Ostreopsis cells typically occurs as summer events. This trend is consistent with the research in the northern Adriatic Sea, where peaks generally occur in September-October. In the Ligurian Sea, peaks are observed in mid-summer, toward the end of July. Studying the growth trend of Ostreopsis cells in Mediterranean areas reveals that the highest abundance can occur from spring to fall [6, 25].
In the northern Adriatic Sea in the Conero Riviera (Ancona, northern Adriatic Sea) blooms of O. cf. ovata have been constantly reported between the end of the summer and the beginning of the fall since 2006 [6, 26]. This temporal pattern suggests that specific environmental conditions during this period may favor the development of the Ostreopsis cells. Several studies have shown the importance of hydrodynamics on the development of Ostreopsis cf. ovata blooms [3, 6]. Moderate waves can cause cells to settle and rough seas and strong wind would rather favor cell dispersion, which reduces the cells’ growth [3, 16]. On the contrary, relatively low wind intensities were sources of matters necessary for Ostreopsis growth [27–30].
The abundance of Ostreopsis cf. ovata in our study reached a value of 6.96 × 10³ cells/l. This finding was similar to research in the south-eastern Mediterranean Sea (Gulf of Gabès), where the maximum concentration was in fall during October (5x 10³ and 7 × 10³ cells/l) and No-vember (8 × 10³ cells/l). In the Gulf of Gabès the highest abundance of Ostreopsis (7 × 10³ cells/l) was reached at temperatures between 22.5 and 30 °C, which is similar to our study [20]. The abundance of Ostreopsis cf. ovata in the coastal areas along the Gulf of Gabès showed a seasonal trend, as previously noticed in other temperate areas in the Mediterranean Sea [17, 20].
Along the coasts of the Ligurian and Catalan Seas, the first peaks of Ostreopsis cells are typically recorded in mid-summer (July), with a second bloom often occurring in fall [27]. In the Northern Adriatic Sea, blooms tend to ap-pear later in fall, between September and October [9]. These findings suggest that temperature has an important role in the occurrence of Ostreopsis cf. ovata blooms, out of simple growth patterns correlated with increasing temperatures.
Sea depth and substratum also have a specific role in studying the occurrence of blooms, as Ostreopsis spp. cells predominantly grow in shallow waters, and high abundances have been observed on macroalgae [3, 31].
Also, among the potentially toxic dinoflagellates, Dinophysis acuta and Phalacroma rotundatum were recorded still with lower abundances (the abundance reached values up to 102 cells/l).
Fig. 2.
Distribution of abundances (cells/l) of total microplankton (TMP) and phytoplankton groups (diatoms and dinoflagellates) during the research period on mussel farms (BK1, BK2, BK3, BK4).
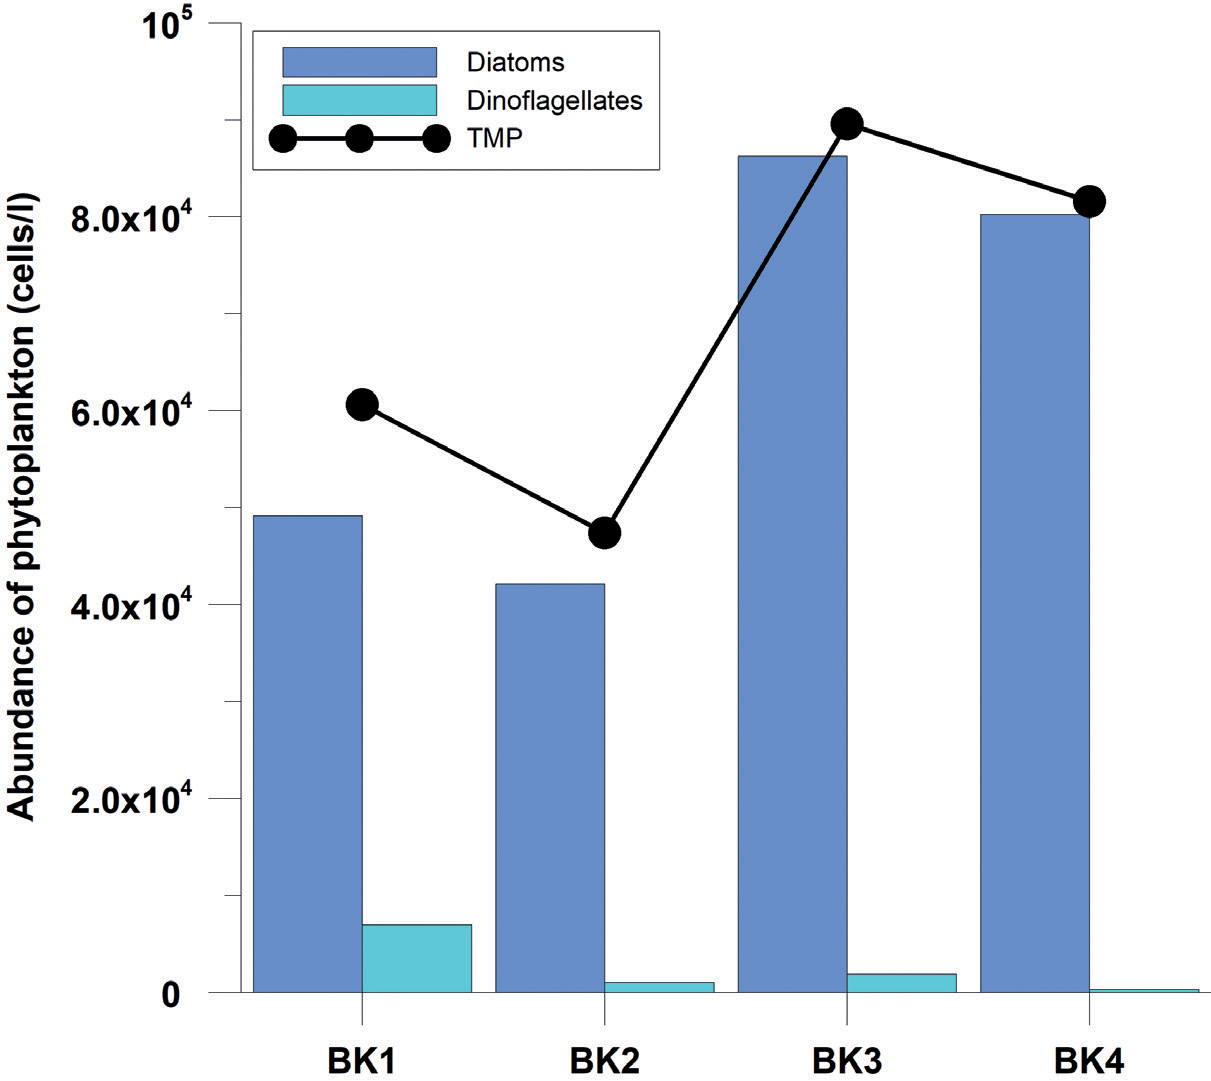
Fig. 3.
Species from the genus Ostreopsis recorded on a Zeiss microscope (Axio Observer A1) in the area of Boka Kotorska Bay-Montenegro (A. magnification is 40X, distance 53.078 µm, scale bar 50 µm; B. magnification is 40X, distance 63.944 µm, scale bar 50 µm).
Our finding is important, knowing that if Ostreopsis species appeared in a frequent “blooming”, it could cause harmful effects on marine benthic communities and human health through skin irritations after direct contact with the seawater, toxic aerosols which cause respiratory problems from inhalation of aerosol [4–6, 27] and contaminated seafood [3, 7, 8, 32, 33].
Conclusion
The reported findings show that the area of Boka Kotorska Bay can be a suitable habitat for Ostreopsis cf. ovata. The occurrence of Ostreopsis cf. ovata in the Boka Kotorska Bay-Montenegrin coast is noticed for the first time, and further investigation will show the occurrence and spread of this species along the entire Montenegrin coast. This record highlights the potential for Ostreopsis to form blooms even under small-scale and localized favorable conditions, emphasizing the need for careful planning of activities in these areas.
Our data should be considered as preliminary, and further detailed studies and analyses of Ostreopsis, particularly on benthic substrates such as macroalgae and rocks, as this species is a benthic dinoflagellate, will be conducted in the future.
Monitoring the presence and abundance of these microalgae is crucial, considering their potential impacts on human health, the ecology of marine organisms, and the negative economic effects on fisheries, aquaculture, and tourism. Such monitoring efforts are essential for prevent-ing risks to both human and environmental health.

