


Introduction
Numerous land-use changes and utilization, such as land conversion, agriculture [1] urban settlements, and industries, lead to land degradation and biodiversity loss, either at the species to ecosystem levels [2–4]. Ecological restoration is a project to accelerate ecosystem recovery of degraded areas by restoring community structure, species composition, and ecosystem functions [5, 6]. In general, the establishment of plant cover is the primary objective of the programs [7]. The establishment of plant cover is important, making the selection of plant species a crucial stage in initiating a restoration project.
The selection of plant species for restoration should consider ecosystem sustainability and current environmental changes. Utilizing native plant species, especially endemic and endangered ones, is strongly recommended as they provide historical references for the habitat. A multi-criteria approach can be employed in selecting plant species for restoration, taking into account both ecological and socioeconomic aspects [8]. In recent decades, there has been an urgent need for management authorities to conduct plant trait profiling and assessment. This is essential for selecting plant species with high ecological establishment capacity, performance, and competitive ability in ecosystems during restoration or rehabilitation programs [9–12]. The selected species should also demonstrate adaptability to water and temperature stresses [13], resistance to herbivory and flame disturbance, and the ability to outperform other species [14]. Moreover, they should possess the capability to resist invasive species [15, 16].
Plant selection for constructing the recommendation system for effective land restoration of degraded areas could be established by considering plant traits that demonstrate the advantages of plants to ecosystems [14, 17–19]. These traits encompass a range of characteristics, including morphological, eco-physiological, biochemical, socioeconomic, and reproductive factors that may be associated with multiple biological pathways and their services to ecosystems [8, 19]. Several leaf traits were suggested as proxies for the ecological function of carbon assimilation, water relations, and energy balance such as SLA (Specific Leaf Area), LDMC (Leaf Dry Matter Content), leaf thickness, and leaf nutrient [20]. SLA represents area-based photosynthetic activities. Other leaf traits, such as stomatal characteristics, nitrogen levels, and chlorophyll content, are also essential for assessing the eco-physiological profiles of plants [21]. Several leaf traits are also proxies of nutrient uptake and photosynthesis, which could be indicated by leaf nitrogen and chlorophyll content [22]. Plant traits showed a complex interaction effect rather than a single impact; therefore, species may possess a combination of response-and-effect traits that matter to the ecological process [23].
In most developing countries, the plant selection processes for restoration were rarely implemented, because the research which serves as a starting point for the selection process is still limited [24, 25]. Previously, [26] proposed a list of local species for restoration based on the carbon sequestration capacity and society’s preferences for plant species for restoration using questionnaire methods. [27] profiled ten woody species that have ecological adaptation to dry environments based on leaf and photosynthetic characteristics. To support natural biodiversity and ecosystem sustainability, proposing high-performed local plant species is preferable, including the native and introduced plants in natural forest areas in a targeted restored environment [28].
Plant trait-based profiling and the development of a framework for trait comparison are still rare to be conducted either for researchers or the management of restoration programs in Indonesia. Here, we applied a low-cost and affordable method to select and recommend highly performed and adaptive woody plant species. We focused on eco-physiological leaf traits that will be used to predict plant survival rates during restoration stages. The study on the variation and correlation of leaf traits across plant species contributes to ecological perspectives on plant life history strategies in tropical Malesian regions. Plant profiling and role prediction of plant species that have high growth and advantageous eco-physiological strategies will be highly implemented for successful land restoration.
Materials and Methods
We investigated leaf traits of twelve local woody plant species using 2-year-old seedlings under a controlled condition. These traits are SLA, LDMC, total chlorophyll content, LNC, stomatal density, and aperture size. We also examined the correlation between these measured traits.
Plant Materials
A total of twelve species, including ten native and two exotic plant species to the Indonesian region (Ficus religiosa and Swietenia macrophylla), were used in this research (Table 1). All studied local species (10 natives and 1 exotic species) are broad-leaved-woody evergreen species, while one exotic species (S. macrophylla) is a broad-leaved woody semi-deciduous species. These twelve plant species were chosen based on the suggested list by [26, 29], which selected plant species based on society and stakeholders’ preferences for restoration and rehabilitation programs. Two exotic species were chosen to compare leaf traits between native and exotic plant species. Plants were propagated and collected in Purwodadi Botanic Garden-Indonesian Research and Innovation Agency (BRIN), East Java, Indonesia, both in adult and seedling stages. Three plants were used for each species for replicability. The information on plant species, habitats [30], and distribution ranges either native or introduction ranges [31] are presented in Table 1.
Table 1.
Species names, local names, habitats, and distribution ranges of studied plants.
Leaf Traits Measurements
Specific Leaf Area (SLA) and Leaf Dry Matter Content (LDMC)
Measurements of Specific Leaf Area (SLA) and Leaf Dry Matter Content (LDMC) were carried out on 2-year-old seedlings using destructive methods, as suggested by [32]. Three plants were used as a replication for each species. Five healthy leaves of each plant were selected and harvested. Leaf area was measured using ImageJ [33]. LDMC was obtained from the dry-oven weights of leaves at 80°C until constant dry weight. Leaf samples were weighed using an analytical balance in each plant species with three individuals as replication. SLA value is the ratio of leaf area value and leaf dry mass (cm2/g).
Stomatal Density (SD) and Stomata Aperture Size (SA)
Stomata observations were carried out using Scanning Electron Microscope (SEM) procedures [34]. Three plants were used for each species for replicability. In the SEM procedure, the leaves were cut into 5x5 mm sizes and excluded the main and secondary leaf veins. The samples were observed using SEM (FEI type Inspects 25) in the magnification of 500–5000 times. The number of stomata was counted from the magnified epidermal tissue areas (square millimeters). The stomatal density was calculated as density per square millimeter. The stomata aperture size was determined by measuring the length of the opened area of the stomata.
Total Chlorophyll Content (CCM)
Total chlorophyll content was measured using CCM-200 plus Chlorophyll Content Meter on mature leaves. Three plants for each species were used as replication and 5 leaves of each plant were sampled. Three sites of leaf surface, i.e. apex-near, middle, and base-near leaf sites, were selected as measurement points to obtain representative chlorophyll content data.
Leaf Nitrogen Concentration (LNC)
Leaf nitrogen concentration was measured at the Soil Laboratory, East Java Agricultural Technology Study Center (BPPT), Malang, using the Kjeldahl method [35]. Three plants for each species were used as replications. Two hundred grams of leaf for each plant were sampled and dry-oven baked. Leaf Nitrogen Concentration (LNC) expressed in mg/g was obtained from the calculation of Nitrogen concentration (%) and the leaf dry mass. Whilst, leaf dry mass was calculated from leaf area (mm2) multiplied by Specific Leaf Weight (SLW) and measured as mg/cm2.
Data Analysis
First, we conducted a normality test to assess whether the data were normally distributed or not. Then, a one-way analysis of variance (ANOVA) and Tukey’s test were conducted to compare leaf traits among plant species at a confidence level of 95% (α ≤ 0.05). Pearson’s correlation tests were performed to identify the correlation between two leaf traits at a confidence level of 95% (P ≤ 0.05). Normality test, ANOVA, Tukey’s test, and Pearson correlation test were performed in R 4.1.0 [36]. Principal Component Analysis (PCA) was conducted to eliminate weak leaf trait predictors on high plant performances for land restoration. The PC analysis was performed using the statistical software PAST 4.0 [37]. High-performance characteristics, which are shown by high SLA, low LDMC, low LNC, and low SD, are used as criteria for selecting plant species utilized in the restoration programs.
Results and Discussion
Variability of Leaf traits Among Species
Eco-physiological traits showed variability across plant species [38]. There were significant differences in all six-leaf traits across the twelve selected plant species based on the ANOVA test (Fig. 1). The significant differences in all six-leaf traits among twelve plant species in this study indicate how the growth strategies of plants vary across species in tropical habitats. Although there is evidence of infra-specific variation in several plant traits which indicated plasticity and the influence of environmental gradients [39], these plant traits are useful to distinguish plant types based on growth and assimilate allocation strategies at the specific level.
In terrestrial ecosystems, SLA is thought to be a reliable proxy for indicating a plant’s photosynthesis, growth rate, and performance in its environment. The higher the SLA value, the higher the photosynthetic activities will be. It ranges from 6.636 to 2040.816 cm2/g of all life forms [32, 40, 41]. Ficus religiosa had the highest SLA value in this study relative to other species. SLA of F. religiosa widely varies between samples, which indicates infra-specific plasticity [39]. This could be possible because this species has a wide distribution range. On the other hand, an endemic species Diospyros celebica had the lowest SLA value, which was not significantly different from the other three native species, i.e., Durio zibethinus, Garcinia dulcis, and Arthocarpus heterophyllus.
The recorded SLA of tropical plants ranges from 90.5 to 298.5 cm2/g [25], and 29.38 to 88.55 mm2/mg for endemic species Zanthoxylum acanthopodium [24]. Therefore, the SLA of F. religiosa in this study was considered as high compared to those of other species and the global SLA record of plant species. The high SLA indicated a strong plant competition in resource uptake, particularly at the maximum use of sunlight. On the other hand, species with the lowest SLA (D. zibethinus, G. dulcis, and A. heterophyllus) did not always necessarily indicate poor performance. It might show high survival rates on degraded land with drought and less fertile soil conditions [42]. Moreover, the exotic species Swietenia macrophylla showed a relatively high value of SLA. This indicated that the range of SLA value among the native species was relatively narrow, while those of the exotic species were relatively high.
LNC of the studied species ranged from 0.004 to 0.135 mg/g. The LNC of Protium javanicum was 0.004±0.00 mg/g, which was significantly lower than that of other species. On the other hand, A. heterophyllus had the highest LNC value with 0.135±0.001 mg/g. Different growth strategies between native and exotic species are also indicated by SLA and LNC. Exotic species S. macrophylla had relatively high SLA but low LNC value. Whilst, the native species D. celebica and D. zibethinus had the lowest SLA value, yet relatively high LNC. This SLA comparison between native and exotic species indicates that exotic species commonly outperform natives [43]. However, there are possibilities that native species may perform as high as exotic and even invasive species.
In general, the LNC value is highly associated with the rate of photosynthesis, which indirectly influences plant development [21, 44]. In this research, the species with the highest LNC was A. heterophyllus. A species with high LNC and SLA values will have a short life span and will accelerate the nutrition cycle in the ecosystem [45, 46]. However, it should be emphasized that the LNC value strongly depends on environmental conditions, such as soil, humidity, and temperature [21, 47]. Moreover, the use of A. heterophyllus will contribute to fast soil nutrient recovery in a restoration.
In contrast to the SLA, the LDMC of F. religiosa was the lowest compared to other observed species. Species with high LDMC values will be more resistant to herbivores or wind disturbances [21]. LDMC is a plant trait that describes the nature of a species’ resource-conserving strategy [48, 49]. As a result, Cynometra schefferi, which had the highest LDMC value of all the species studied, was likely to exhibit wind and herbivore disturbances resistance.
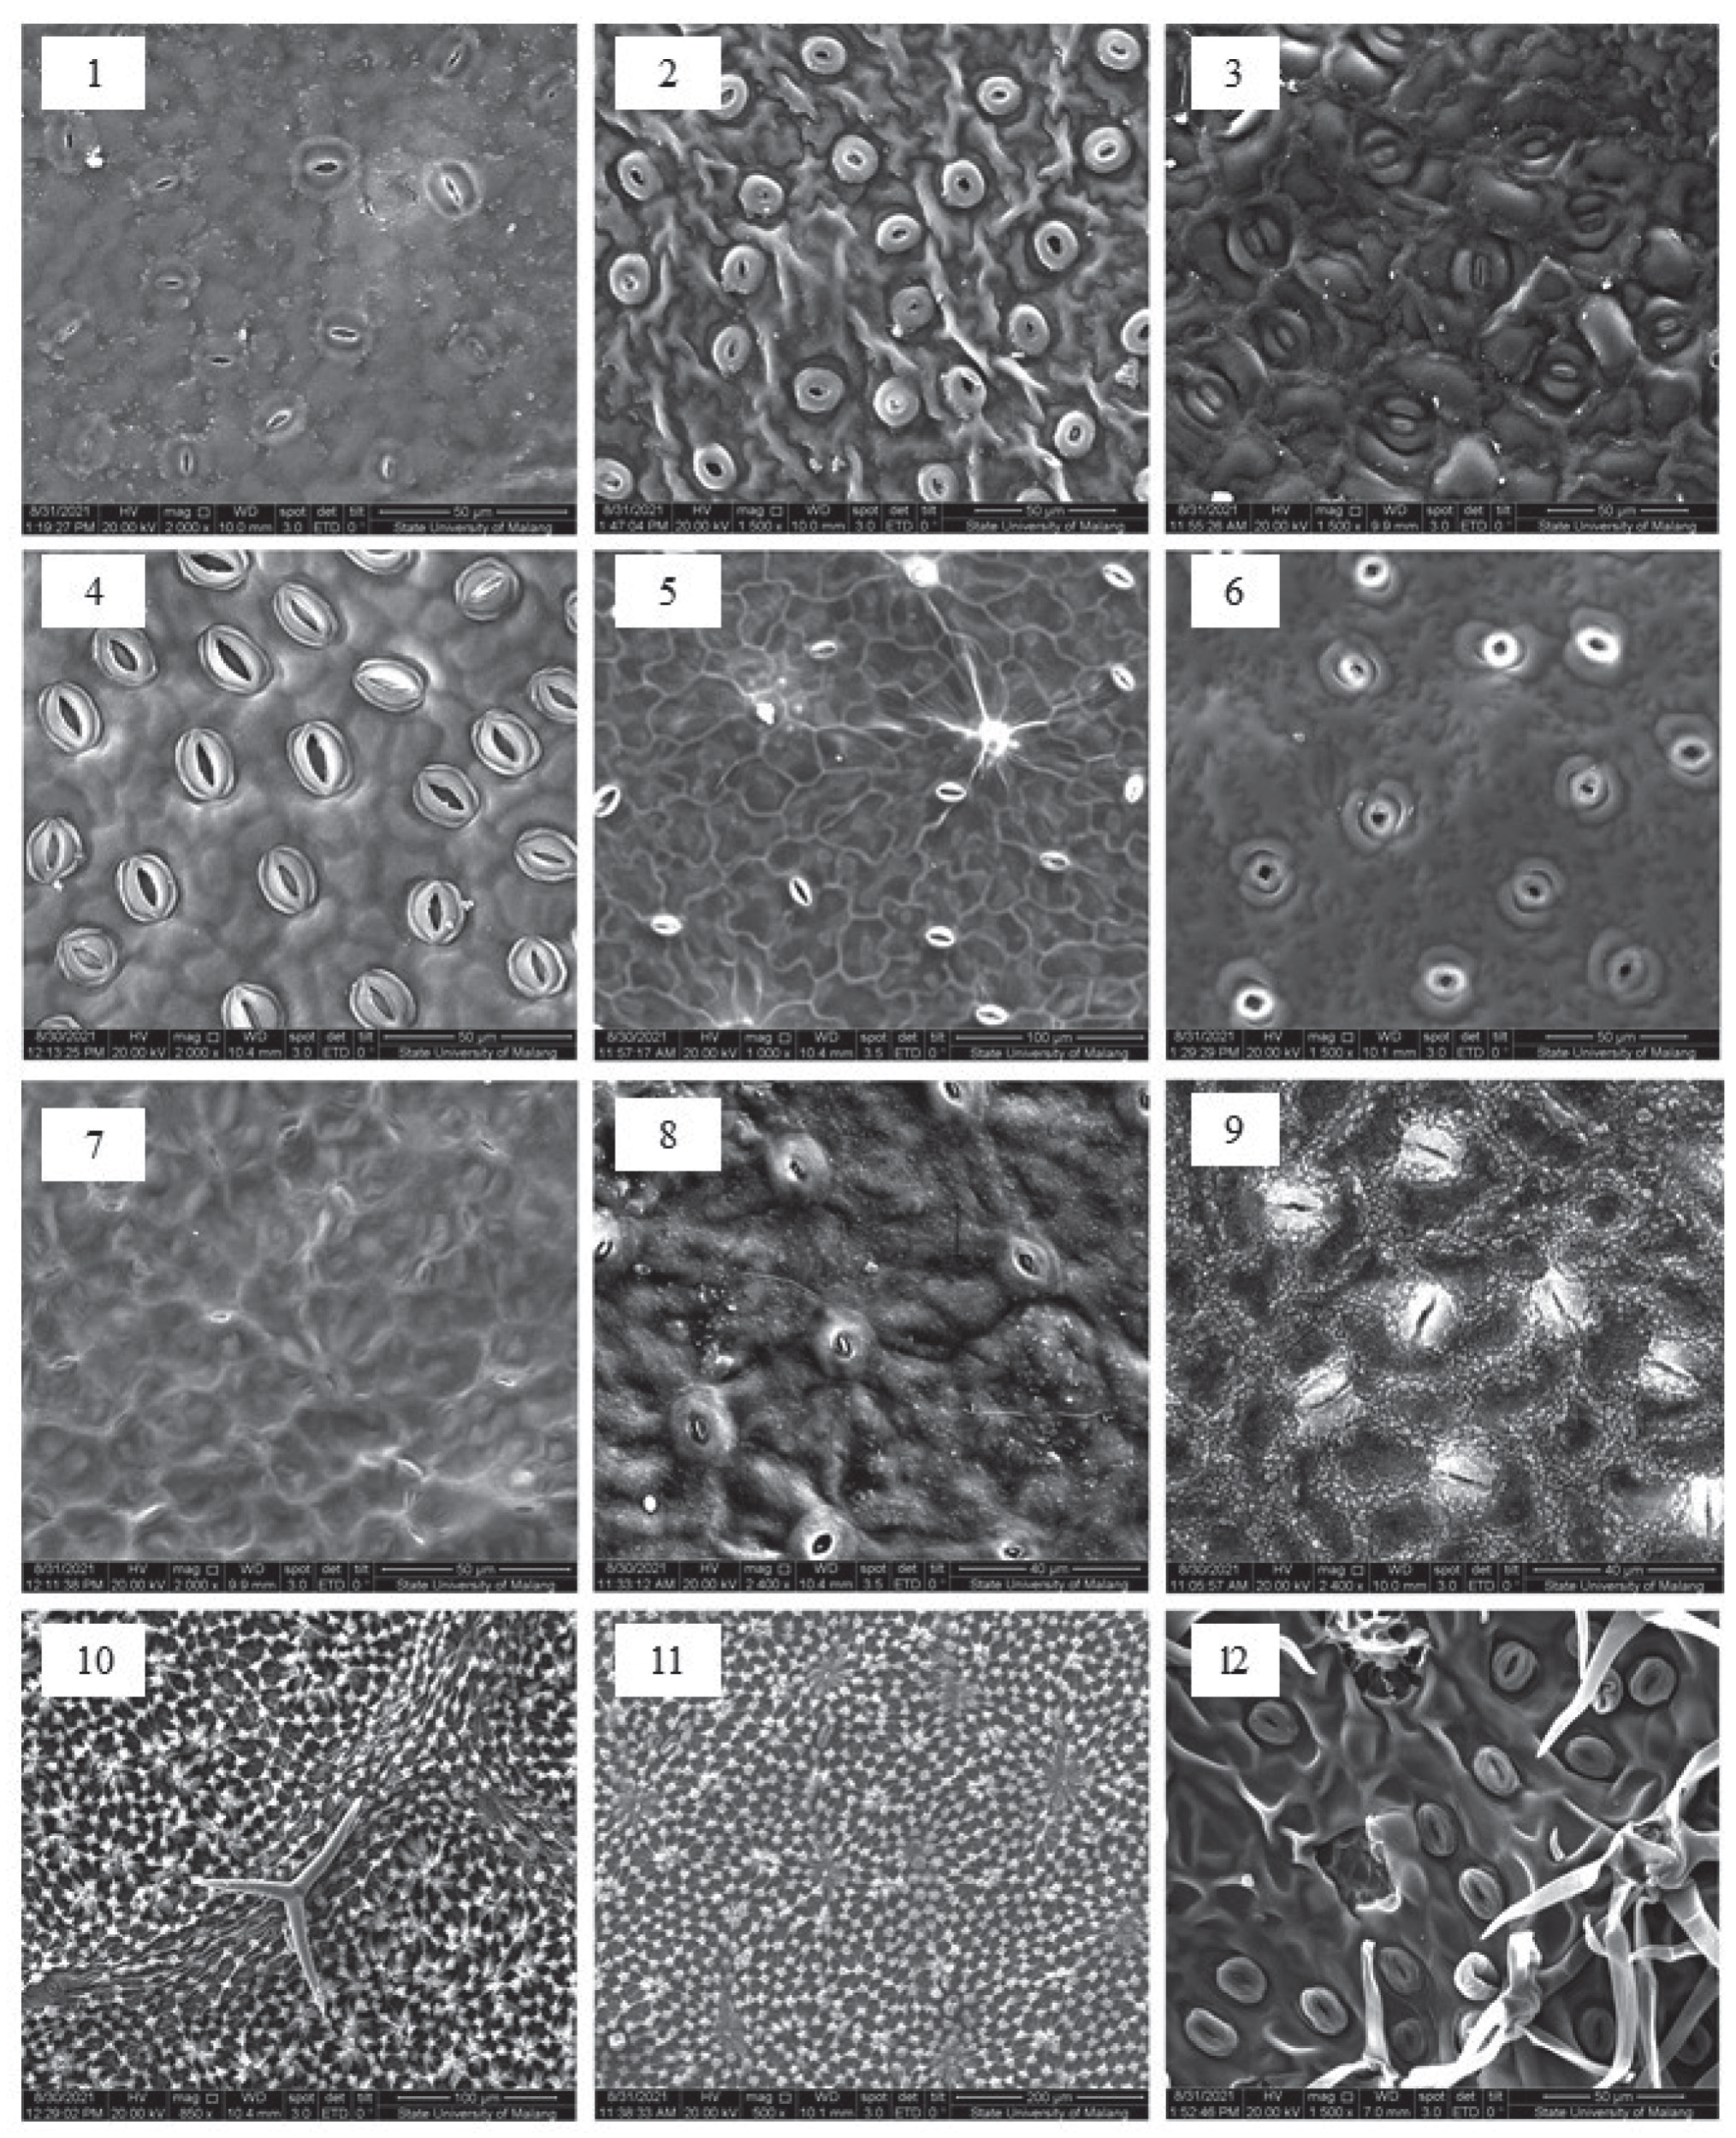
The variability of stomatal traits demonstrates the different growth strategies on leaf gas exchange and water loss regulation between native and exotic species (Fig. 2). The exotic species S. macrophylla showed the lowest value of stomata aperture size but with relatively high stomatal density. In contrast, the native species D. celebica had the lowest stomatal density and the largest stomata aperture size. The high stomatal density of exotic species S. macrophylla represented high photosynthetic activity, fast growth rate, and water loss of plants and soil [27, 50]. Planting this species in restoration may negatively affect the surrounding restored ecosystem and water conservation.
Correlations, Trade-Offs between Leaf Traits and Life History Strategies
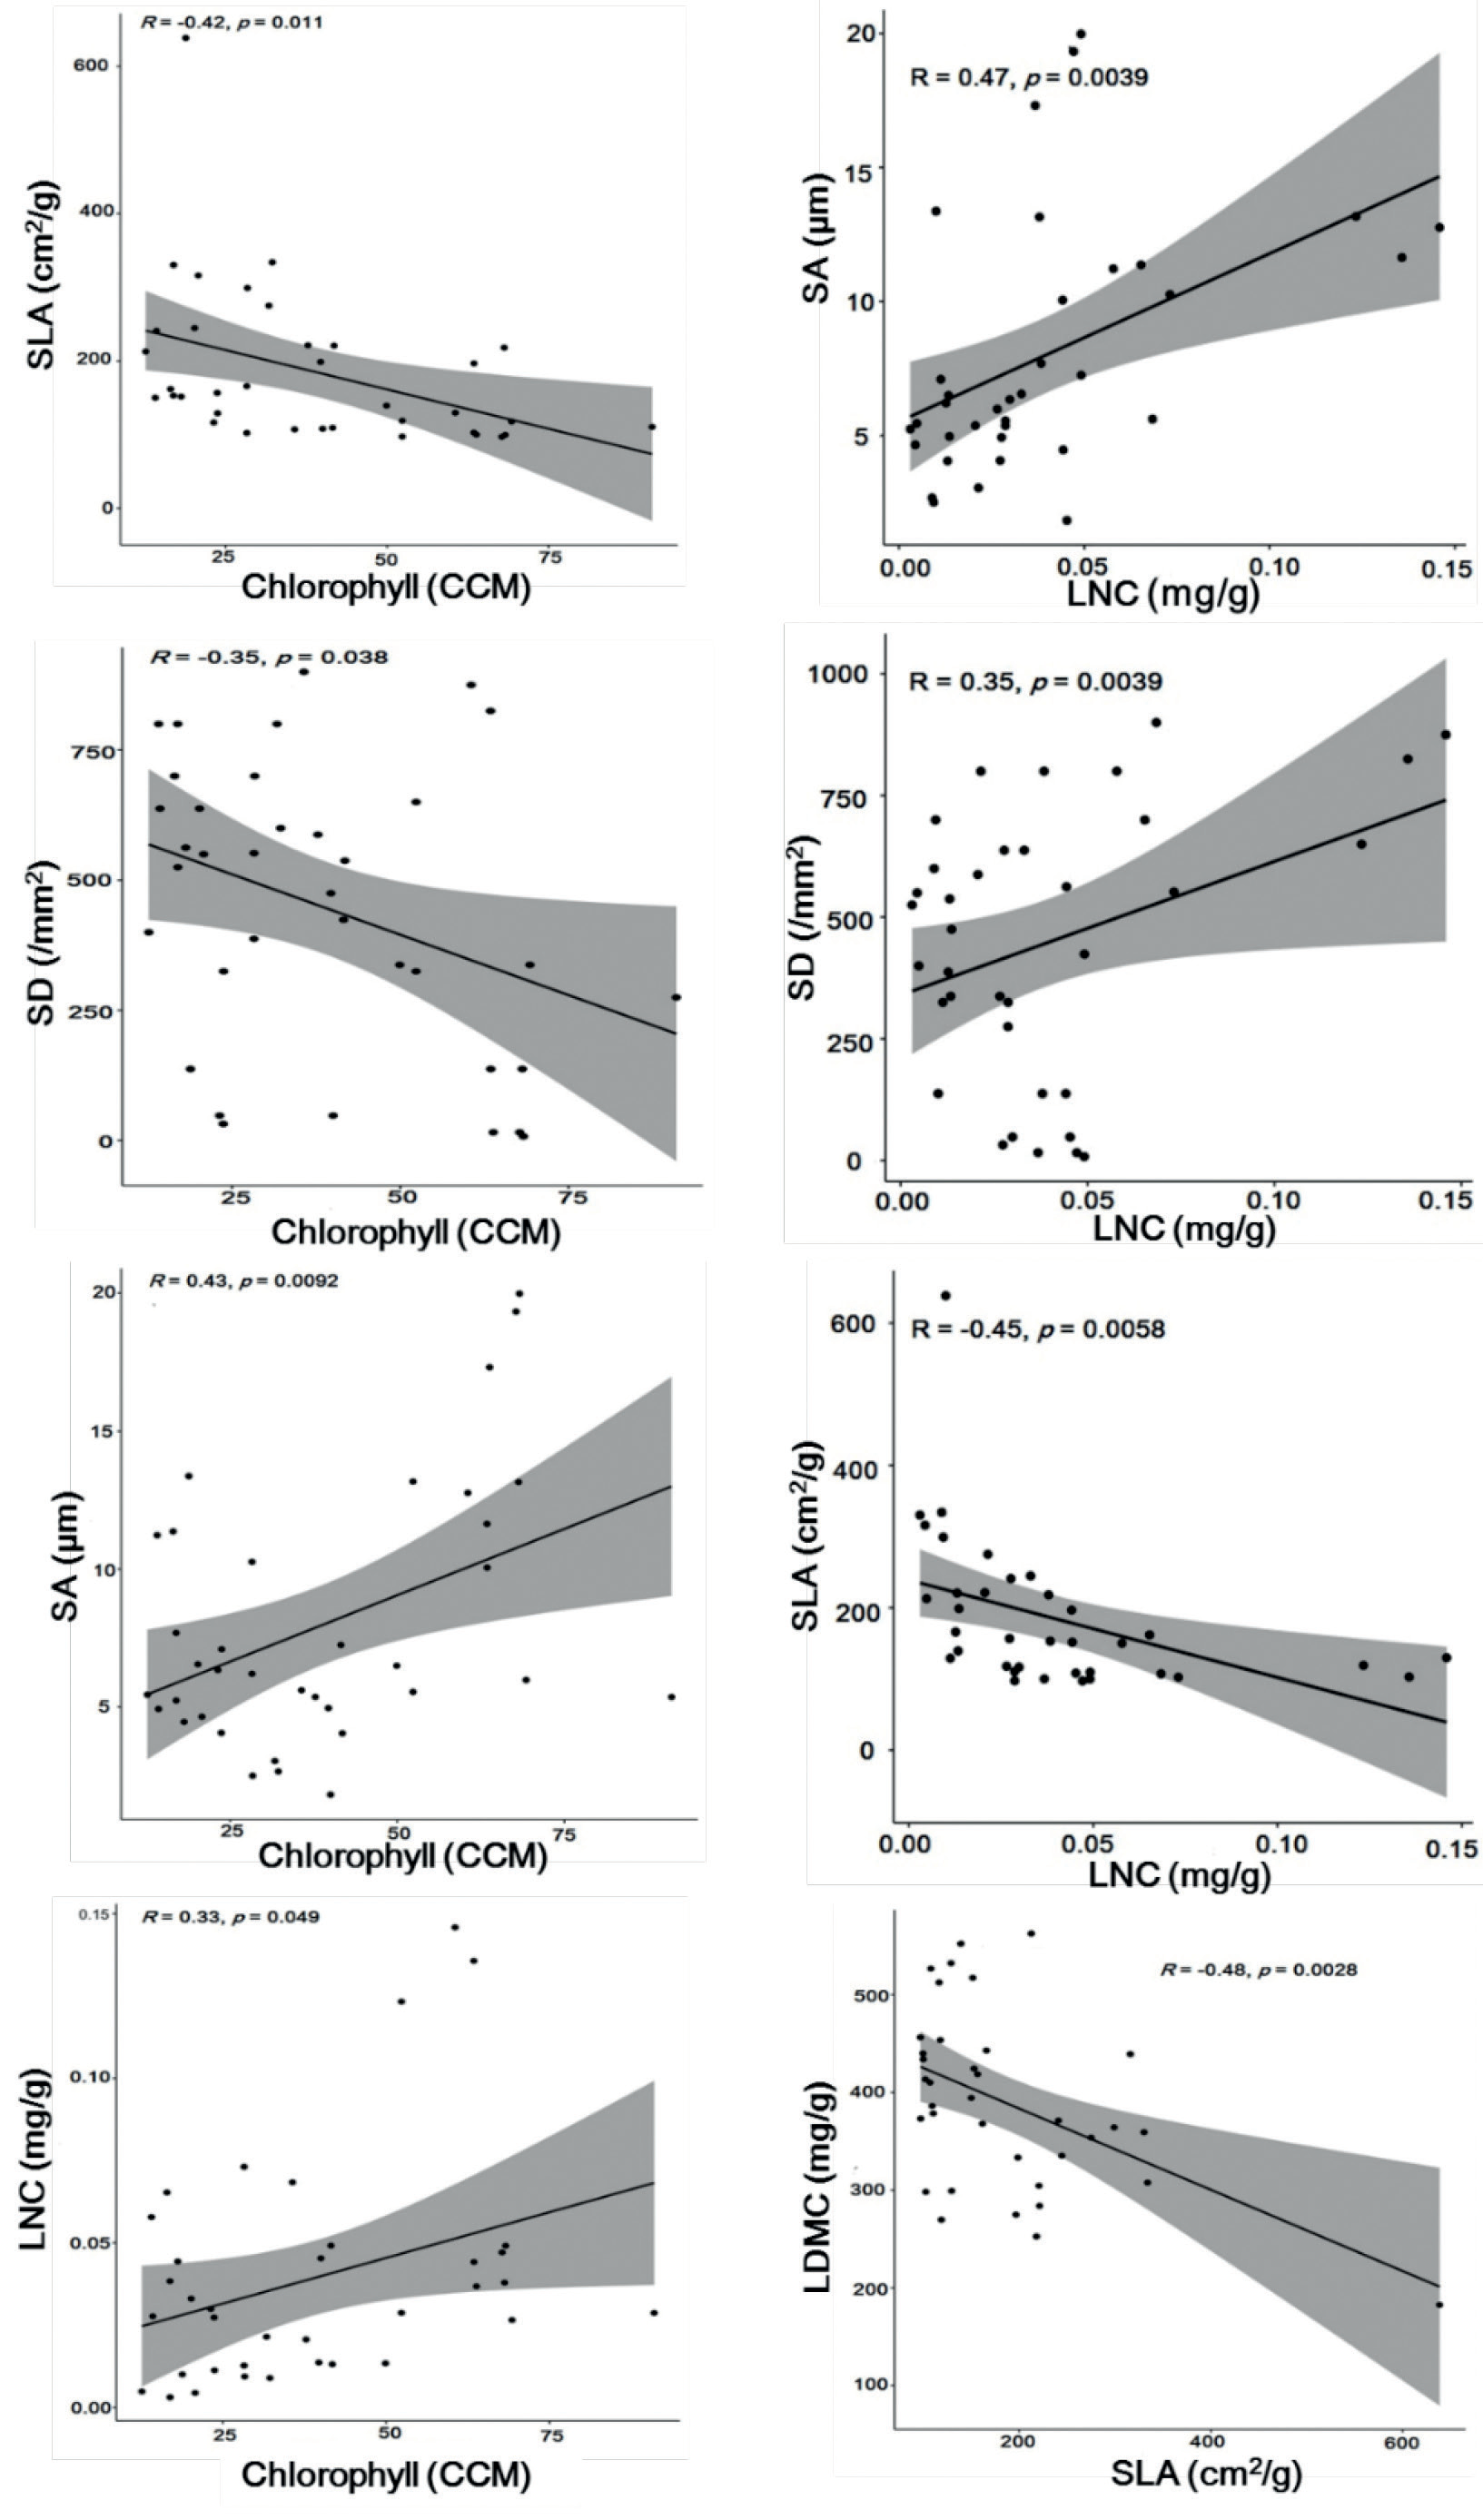
We investigated the correlation of measured leaf traits among plant species to identify the bivariate relationship between leaf traits. We extracted essential correlations between leaf traits at P<0.05 and detected eight significant correlations (Fig. 3 and Table 2). A negative correlation between two particular functional leaf traits tends to demonstrate a trade-off in the life history strategy of plant species in adapting to a challenging environment [51]. In this study, negative correlations were detected between LNC with other important traits related to growth and photosynthesis, i.e., SLA and stomatal density. This functional plant group takes advantageous strategies to obtain rapid growth by increasing photosynthetic activity and foliage display, but tends to decrease nitrogen allocation into leaf organs. The high level of N may not be advantageous for plants since it could increase herbivory through the attractiveness of high nutrition [52, 53]. A negative correlation between SLA and LDMC may demonstrate a trade-off between leaf traits that relate to the level of flammability. According to [21, 54], flammability could be predicted through the dry matter content of plant leaves (LDMC). The studied plant group demonstrated the life strategies to maximize productivity and simultaneously implement flame and herbivory risk avoidance mechanisms.
Fig. 1.
Box plot graph of leaf trait values of studied species. Species 1–12 were listed according to Table 1. Different letters represent significant differences between species according to a post hoc Tukey test (p< 0.05).
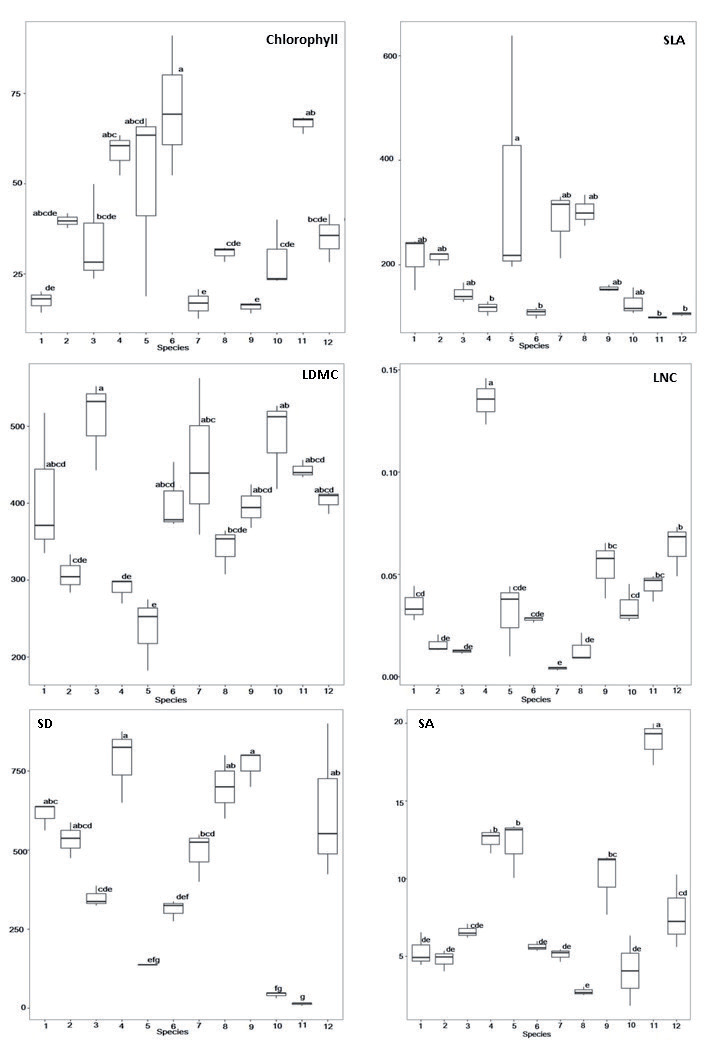
Fig. 2.
Scanning electron micrographs showing the density of stomata on the abaxial surface of 12 species studied, which are listed according to Table 1.
Chlorophyll content had a positive correlation with nitrogen level and stomata aperture size as well as nitrogen level, which had a positive correlation with aperture size. Further, chlorophyll content was supported by stomata aperture size, but not by its density. A positive correlation between chlorophyll content and LNC was revealed by previous studies [55]. The chlorophyll content is influenced by nitrogen level because nitrogen is one of the most essential nutrients for plant growth and serves as a major component of chlorophyll and protein [56, 57]. Nitrogen levels affect chlorophyll content that may influence the development of stomata to maximize gas exchange of photosynthetic activity. Since SLA was negatively correlated with nitrogen level, the increase of photosynthetic capacity might occur in the leaf area scale (cm2). Consequently, when leaves had a large foliage display (high SLA value), leaf nitrogen levels tended to be decreased to develop an adaptation mechanism in protecting leaves from mechanical disturbance, which includes predatory herbivores or flame risks.
Strong Trait Predictor and Recommended Species for Restoration
Among the six investigated leaf traits in this study, strong predictors were preferred as the baseline in the determination of high performance-species in growth and life history strategy, which may be ecologically advantageous for restoration programs. Based on the component analyses, for these twelve studied species contexts, two leaf traits i.e. SLA and LDMC were stronger predictors compared to other leaf traits at a total of variance 70.58% which consist of 45.82% and 24.77% from PC1 and PC2 respectively (Fig. 4). We also arranged the information on ecological attributes that relate to light tolerance based on stomatal density and leaf morphology [58] to predict the role of plant species in restoration (Table 3).
Table 2.
Bivariate combination of six plant traits.
Fig. 3.
Detected significant correlation between studied leaf traits according to the Pearson Correlation test (p<0.05).
Specific Leaf Area (SLA) is widely proven as the best predictor of plant photosynthesis, growth rate, and performances in various habitats and ecosystems [59, 60], which play important roles in plant competition, or even in plant invasion context [21]. The large range of SLA among the species in the global plant and woody plant group itself leads to a wider opportunity to explore and identify native species with higher SLA. LDMC indicates a plant adaptation strategy that relates to the risk of flammability. The lower the LDMC value, the higher the plant species’ ability to avoid destruction caused by a flame in their natural habitats [21, 61]. Wüestr R.O. et al. [62] found that LDMC is a more reliable predictor relative to other plant traits, especially those related to environmental services. Therefore, the result of the study also supports the previous result about the importance of SLA and LDMC in plant functional ecology.
High growth rate and high resistance to flame and herbivory were important criteria in the restoration, indicated by high SLA and low LDMC values, respectively. The resistance to herbivores was also supported by low LNC. The determination of these criteria is consistent with most study results on plant traits carried out on seedlings under controlled conditions [53, 63]. The component of plant growth serves as species attributes rather than measured plant characteristics, which are more influenced by environmental conditions.
We recommend the use of native plant species that had high SLA but low LDMC, which demonstrated high photosynthetic activities and advantageous strategy in decreasing the risk of herbivory at restored habitats (Fig. 4; Table 3). Exotic species Ficus religiosa and S. macrophylla showed high SLA. Numerous study results showed that SLA strongly impacts plant growth rate associated with plant invasive occurrences. Species with a high value of SLA are considered to show a high risk of invasiveness in recipient-restored tropical habitats [64, 65]. Therefore, these two species were less recommended to be planted in restored areas in tropical regions of Southeast Asia. Effective controls of invasive species are rarely in restoration projects because it is long-term and high-cost efforts. Providing basic information through research on intrinsic aspects of plant species could guide successful restoration projects [16].
On the other hand, a native species P. javanicum had a high SLA, higher than those of the exotic species S. macrophylla. Moreover, four species were relatively sun tolerant and had high SLA, therefore were highly recommended as strong-performing pioneers i.e. P. javanicum, S. polyantum, C. vulgare, and A. heterophyllus. Regarding to the light tolerance and SLA value, C. schefferi, G. dulcis, D. longan, and D. celebica were recommended as inserted species in land restoration. Cinnamomum sintoc and D. zibethinus were two sun-tolerant species with relatively low SLA, therefore these two species were recommended as pioneer species on restored land with the intensive control of weeds.
Durio zibethinus with the local name “durian” is a native-tolerant species with a low value of SLA and high stomatal density. This species will be preferable for restoration because of its economic value by producing favored and delicious fruit. Because of the low SLA, as a pioneer plant, this species had low photosynthetic activities that led the plants to sufficiently compete with the weeds and invasive plants on the restored land. The high stomatal density of D. zibethinus indicated that this species might lose water rapidly due to high transpiration rates. Therefore, intensive weed control and regular watering are necessary treatments for this species in restored areas.
Fig. 4.
Principal-component analysis of 6 leaf traits of 12 plant species. Different dots color represent different species.
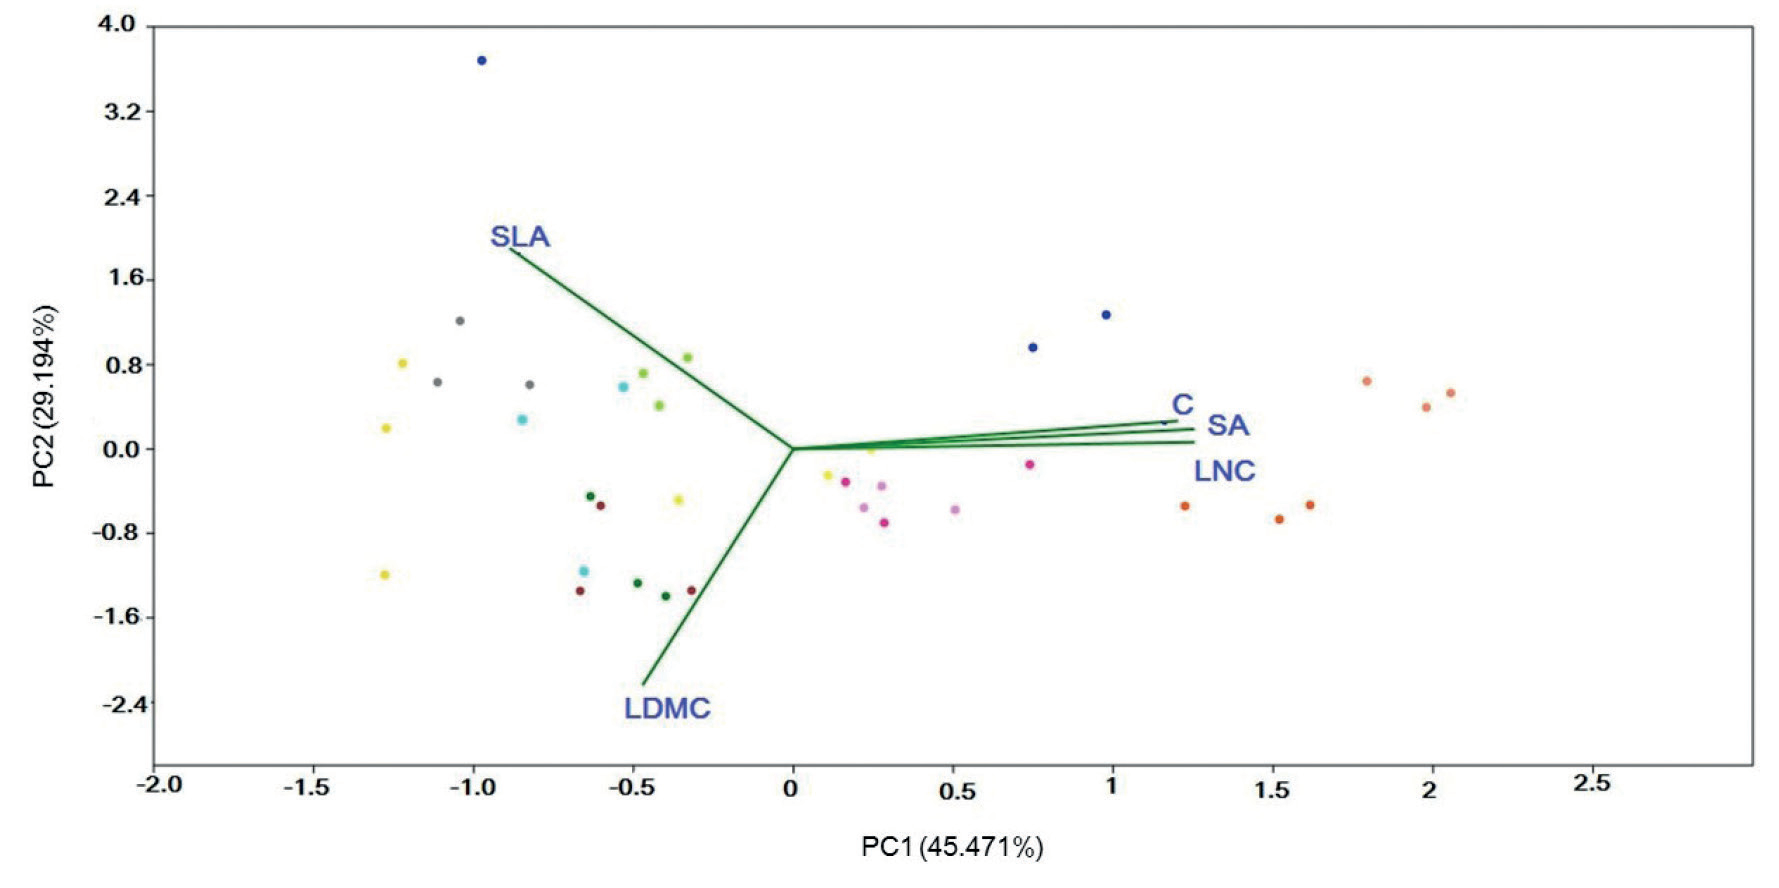
Table 3.
Ecological attributes and predicted role of the studied species on land restoration.
In field conditions, plant growth will be influenced by the nature of plants (shade or sunlight tolerance) and the characteristics of the habitat (shaded or opened environment). Shade-tolerant species could form small leaves to reduce the heat load, but in tropical forests, light-demanding species had large leaves compared to shade-tolerant plants to compete with their co-existing plants. Sun-tolerant species have a high SLA and Leaf Area Ratio (LAR) to increase photosynthetic rates by absorbing more sunlight in a light-limited environment, whereas shade-tolerant species have a low SLA compared to light-demanding species [66]. Plants that grow in shady environments could show a high survival rate by growing slowly since plants develop conservative strategies by sustaining in low-energy environments rather than maximizing net carbon gain in the shade [67].
In some restoration cases, native plant species showed high and moderate growth rates when seedlings were planted in degraded areas with open habitats, plenty of light, and adequate ground cover. Kestari D.A. et al. [68] revealed that native Bornean species such as Shorea balangeran and S. lamelatta were growing well on open degraded land in coal-ex-mined areas. Shorea balangeran was also report-ed to have high survival and growth rates in the restoration of peat swamps in Borneo [69]. In the field situations, SLA, which represents growth rates, could also be positively correlated with plant survival rate likewise revealed by [13].
Conclusions
This study adjusts the manifest to ecological knowledge that eco-physiological traits of plants vary across species. The correlation between two leaf traits, especially SLA, LNC, and LDMC, showed plant trade-offs in plant growth and life history strategy related to herbivory and the risk of flammability. The results strengthen the global perspective on SLA and LDMC as strong predictors in plant performance, which serve as the baseline of plant species selection for restoration. The two exotic species, i.e., S. macrophylla and F. religiosa showed a risk of invasiveness in tropical habitats of Southeast Asia based on sun adaptation and high SLA. Native plant species group in this study, i.e., P. javanicum, S. polyantum, C. vulgare, and A. heterophyllus are recommended as pioneer species in restoration based on sun adaptation and high SLA, with two species, i.e., C. sintoc and D. zibethinus should be accompanied with intensive weeds control, while other native species, i.e., C. schefferi, G. dulcis, D. longan, and D. celebica are recommended as inserted species. Besides, we recommend using of high-performing plant species in restored habitats. We also demonstrate that the study on eco-physiological traits takes an important role in plant species selection, which serves as a critical stage in successful restoration programs.

