

Introduction
During the coevolution with hosts, parasitoids have developed many host-searching strategies to adapt to host escape behavior [1]. Successful parasitoids effectively interpret environmental messages to improve their searching success rate. Learning behavior is an important component of such strategies, and refers to the new behavior and activity mode of the parasitoid [2, 3]. The establishment of learning behavior is related to the specific life history of the parasitoid. Learning is a repeatable and reversible behavioral change that is acquired by and retained in nerve cells [4]. Parasitoids exhibit specific learning abilities at each developmental stage, although the learning environment experienced during the adult stage has the most direct effect. Unconditioned and conditioned stimuli in microenvironments can be associated with and used directly to assist in host-searching [5, 6]. Studies of several insects, including Aphidius gifuensis, Sclerodermus pupariae, Diachasmimorpha kraussii, Nasonia vitripennis and Nasonia giraulti, concluded that botanical volatiles provide important chemical signals in the search for parasitoids. Using environmental signals effectively is important for parasitoids to quickly find an appropriate host and improve search efficiency by odor learning during the early eclosion period [2, 7-9].
Sclerodermus sichuanensis Xiao (Hymenoptera, Bethylidae) is an indigenous species found exclusively in the Sichuan province of China, serving as an external parasitoid of longhorn beetle larvae [10]. This parasitoid has a short development cycle, relatively high fecundity, environment adaptability and host-searching ability. S. sichuanensis has been successfully propagated on a large-scale using substitute hosts and has been applied to the biological control of boring pests, including Aromia bungii, Semanotus sinoauster, Callidium villosulum, Clytus validus, Monochamus alternatus, and Batocera lineolate [11]. However, host-searching ability of parasitoids propagated in the laboratory with a substitute host decrease [12, 13]. We observed that S. sichuanensis displays intricate cognitive capacities in the domains of spatial memory and associative learning. Moreover, S. sichuanensis exhibits exceptional innate aptitude in acquiring and interpreting chemical stimuli emitted by plants. Such cognitive abilities endow S. sichuanensis with the ability to navigate its environment skillfully and respond effectively to fluctuations in its surroundings. Therefore, we hypothesized that provision of information stimuli related to the target pest will increase the target-searching ability of S. sichuanensis when S. sichuanensis is reared on a substitute host. In this study, the learning of S. sichuanensis were examined after experiencing a mixture of longhorn beetle (Anoplophora chinensis Forster) fecula and wood meal followed by successive or simultaneous exposure to two different mixtures of A. chinensis fecula and wood meal. The mutual effects on learning from different experiences of S. sichuanensis will provide a solid foundation for the better use of learning behavior to improve its host-searching ability.
Material and Methods
Odor Source
Odor sources were combined in tests as follows:
I. A mixture of A. chinensis fecula and wood meal from willows.
II. A mixture of A. chinensis fecula and wood meal from Platanus orientalis.
Anoplophora chinensis fecula and wood meal from willows and P. orientalis were collected from Sichuan Agricultural University (103°0′7″E, 29°58′52″N). Fresh mixtures of fecula and wood meal from affected tree trunks were collected daily from 09:00-10:00 am. Collected mixtures were placed in sealed plastic bags (45 cm × 55 cm, Toppits, Minden, Germany) and then stored at 0ºC before use.
Preparation of the Odorous Environment
The odorous environment consisted of 20 g of the respective mixtures of longhorn beetle fecula and wood meal packed with sterile double-layered absorbent gauze into sealed 500 mL wide-mouth bottles.
Collection of Volatiles from Mixtures of Longhorn Beetle Fecula and Wood Meal
We sealed 10 g of odor source I or II into plastic bags (45 cm × 55 cm, Toppits), inserted glass tubes containing 50 mg Tanex-TA adsorbent (60–80 holes; outer diameter 6 mm × 85 mm long, Supleco, Bellefonte, PA, USA) and an activated carbon pipe filter into opposite angles of the bag, connected the inlets and outlets of the air samplers with Teflon tubes, and dynamically collected the adsorbed volatiles for 1 h at an air flow of 0.5 L/min. Then, volatiles were eluted with 5 mL of redistilled diethyl ether (chemically pure, Chengdu Kelong Chemical Reagent Plant, Chengdu, China) and concentrated to 2 mL with N2 for electroantennogram (EAG) determinations.
Test Insects
Adult female S. sichuanensis were reared on yellow mealworm pupae in glass breeding tubes (diameter 7 mm, length 6 cm) in the Provincial Key Laboratory of Forest Conservation of Sichuan Agricultural University. The pupal stage of S. sichuanensis lasts for 20 d. Breeding tubes containing a medium quantity of clean S. sichuanensis cocoons were selected 15 d after pupation in the environmental chamber at 25±1ºC and RH 60%-70%, and emerging adults were collected daily and marked [14].
Learning Behavior of S. sichuanensis from Continuously and Discontinuously Repeated Experience of Odor Source I
We conducted comparisons between four-day-old adults that were exposed to odor source I for three consecutive days and those that experienced odor source I only on the 1st, 3rd, and 5th day. Additionally, we compared four-day-old adults that were exposed to odor source I for one day with six-day-old and eight-day-old adults exposed to odor source I for one day.
The tropism response of S. sichuanensis to the odor experienced in the Y-tube olfactometers was recorded on the second day after treatment. Each experimental treatment is repeated three times, with 30 S. sichuanensis used for each repetition.
Learning Behaviors of S. sichuanensis Experiencing Odor Sources I and II Successively or Simultaneously
Behavioral responses were examined under the following experimental protocols: 1). Adults experienced odor source I at 1 day old for 1 day and their behavioral response to odor source I was determined at 5 days old; 2). adults experienced odor source I at 1 day old for 1 day and their behavioral response to odor source II was determined at 5 days old; 3). adults at 1 day old experienced odor source I for 1 day and then experienced odor source II for 1 day at 4 days old, and their behavioral response to odor source I was determined at 5 days old; 4). adults at 1 day old experienced odor source I for 1 day and then experienced odor source II for 1 day at 4 days old, and their behavioral response to odor source II was at 5 days old; 5). adults at 1 day old experienced odor source I for 1 day and experienced odor source II for 1 day at 4 days old, and their behavioral response to mixed odor sources I and II was at 5 days old; 6). adults at 1 day old experienced mixed odor sources I and II for 1 day and their behavioral response to mixed odor sources I and II was determined at 5 days old; 7). adults at 1 day old experienced mixed odor sources I and II for 1 day and their behavioral response to odor sources I was determined at 5 days old; and 8). adults at 1 day old experienced mixed odor sources I and II for 1 day and their behavioral response to odor source II was determined at 5 days old.
Each experimental treatment is repeated three times, with 30 S. sichuanensis used for each repetition.
Tests of Searching Behavior of S. sichuanensis in the Laboratory
Willows and P. orientalis trunks previously unharmed by A. chinensis were sawn into blocks (3 cm in diameter and 15 cm long). Both ends were sealed with paraffin to reduce water loss. A 3 cm × 4 cm section of bark was removed, and a 2 cm × 3 cm artificial worm path was created in the xylem in the middle of the area using an engraver. Two or three A. chinensis larvae obtained from willows or P. orientalis were placed into the artificial worm path, and then the removed bark section was put back and secured with pushpins. Tests were carried out at 25±1ºC after inoculating for 5 days with freshly discharged fecula and wood meal.
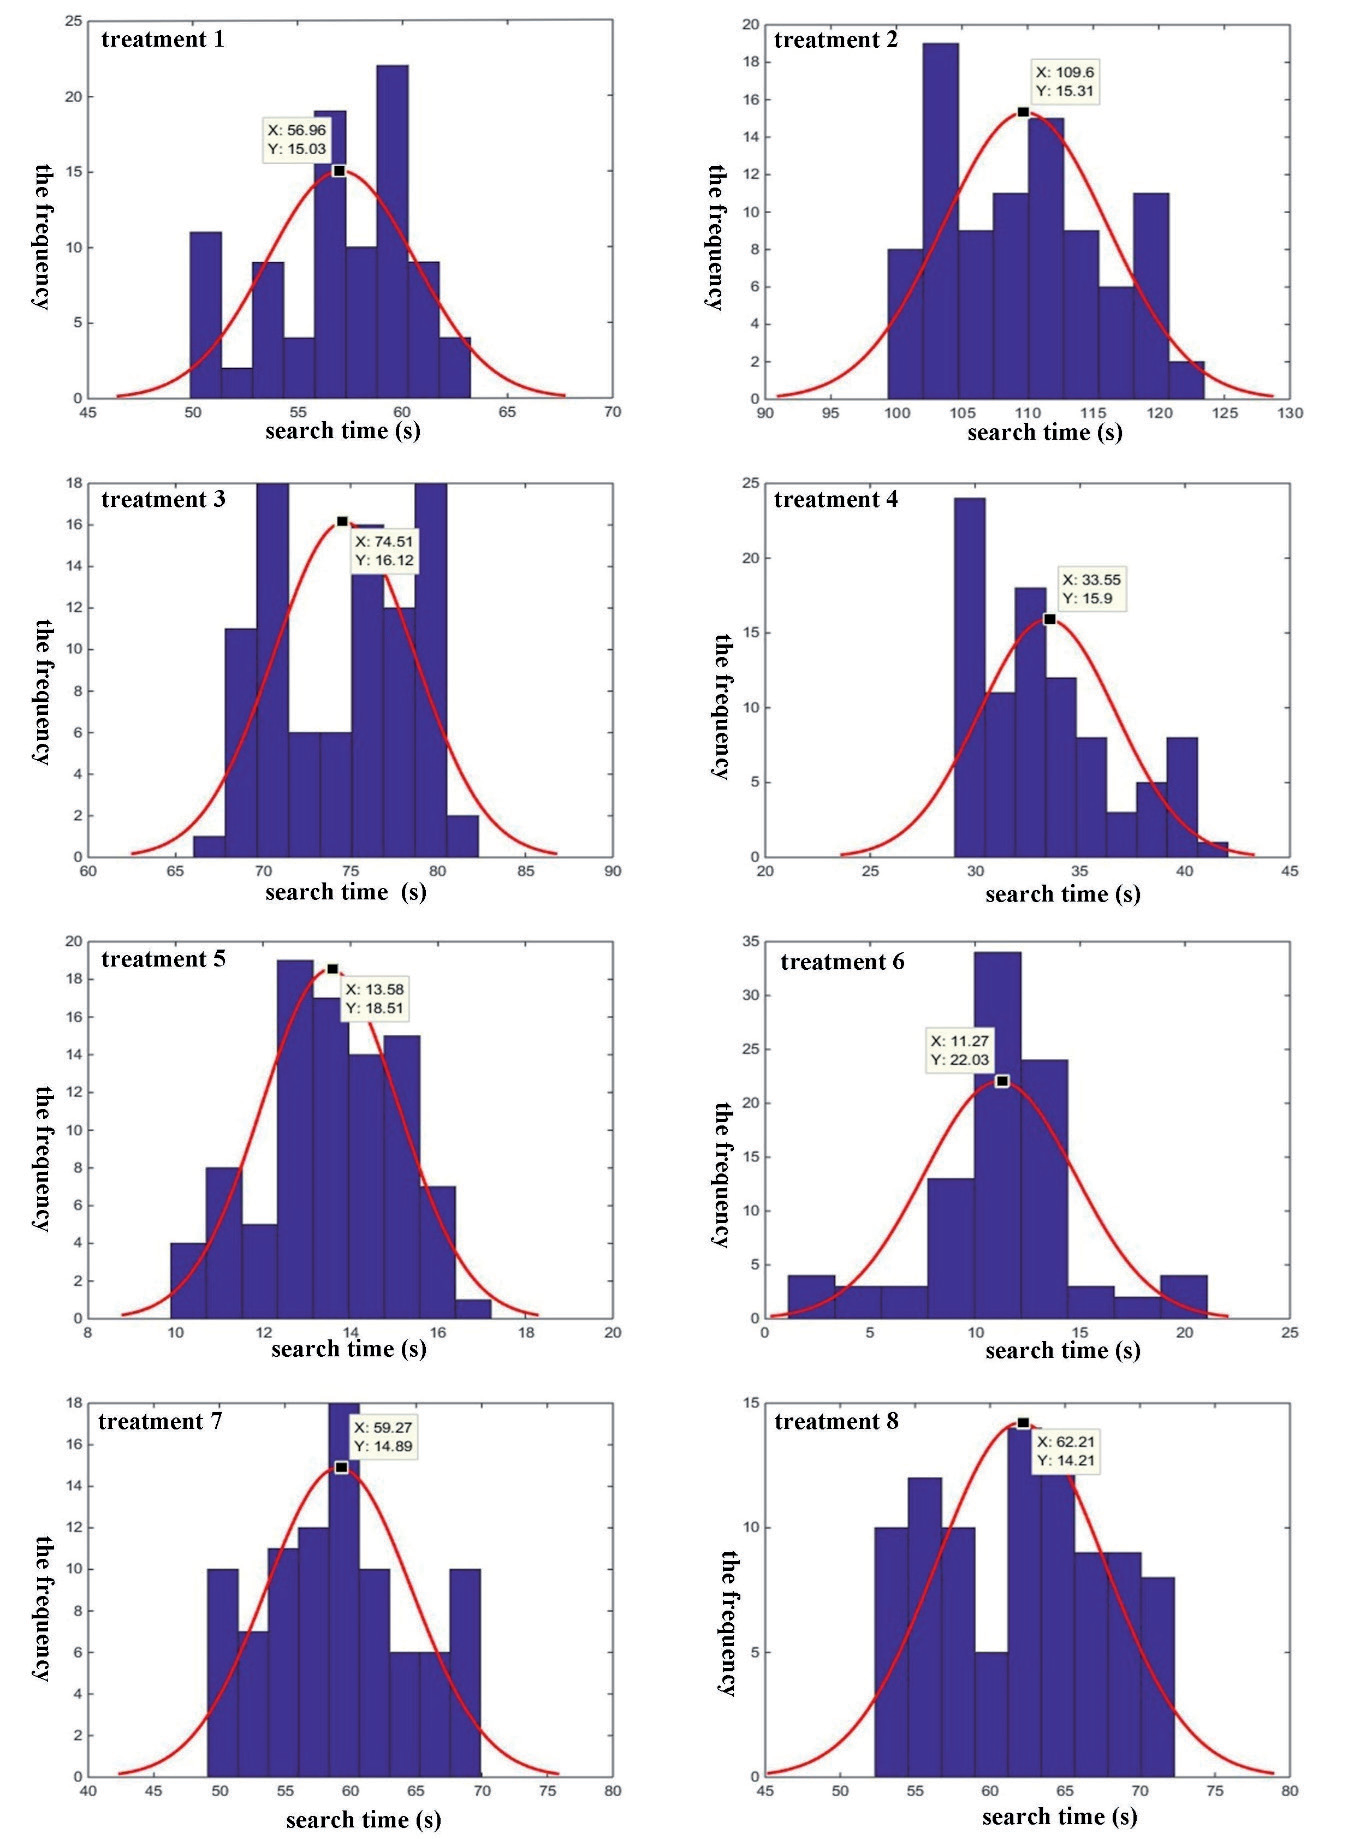
Responses of S. sichuanensis were examined as described in 2.6. Two wood blocks were placed into a 50 cm diameter glass desiccator (for mixed I and II odor sources, one willow block and one P. orientalis block). S. sichuanensis adults were released at a fixed position of the desiccator at 25±1ºC. A search was deemed successful when the S. sichuanensis entered the bark (for the mixed odor source, either the willow block or the P. orientalis block) and the search time recorded. The experiment consisted of eight distinct treatment conditions, each with three replicates. With 30 S. sichuanensis used for each repetition.
Bioassay of Behavioral Responses
A Y-tube olfactometer was used to determine behavioral responses of the parasitoids to the odor. The olfactometer (inside diameter 1 cm) consisted of a long arm (10 cm) with a standard ground opening and two side arms (5 cm) at an angle of 75°. The side arms were connected to 300 mL volumetric flasks with Teflon® tubing. One volumetric flask contained the odor source and the other was empty. The volumetric flasks were connected to a distilled water humidification bottle (300 mL) and an air purification bottle (500 mL) containing activated carbon using Teflon® tubing, and then to the outlet of an air pump (flow rate 0.5-0.6 L/min).
Tests were conducted between 08:00 am and 12:00 pm at 25±1ºC. For the bioassay, parasitoids were introduced into the long arm of the Y-tube, and timing commenced when it had moved 2 cm into the arm. Each parasitoid was observed for 5 min. If it entered 3 cm into a side arm and remained there for >1 min, it was recorded as choosing the odor; otherwise, it was recorded as making no choice. After tests were conducted on five parasitoids, the positions of the two arms of the Y-tube were swapped to eliminate possible influence of the pipe arm position on parasitoid behavior. When each treatment finished, the Y-tube olfactometer was changed; the Y-tube, Teflon® tubing, and the volumetric flasks were thoroughly washed with alcohol and allowed to dry naturally. Y-tubes and volumetric flasks were then heated to 100ºC for 24 h to eliminate residual odors from the treatments.
EAG Determinations
EAG determinations were made using an IDAC-2 signal acquisition system (Ochenfels SYNTECH GmbH, Buchenbach, Germany). An insect pin was used to remove the terminal 1-2 segment(s) of the scape of an antenna from the head of S. sichuanensis. The segment(s) were fixed onto the preamplifier (gain 10×) electrode with conductive gel (SpectraR360, San Francisco, CA, USA) at a distance of 1 cm from the odor outlet. A micro-sampler was used to drip 2 µL of the odor source uniformly onto a 5 cm × 0.5 cm filter-paper strip. The strip was placed into a 10 cm long sample tube connected to the odor stimulus control device, and when the baseline was stable, stimulation was started. Stimulation occurred for 0.5 s at intervals of 30 s, which allowed complete recovery between stimuli. Each antennal sample was stimulated five times. Redistilled n-hexane was used as the control. The average of the observed values for each sample was divided by the value obtained from two control determinations to generate the relative EAG response. Each experimental treatment is repeated three times, with 10 S. sichuanensis used for each repetition.
Data Statistics and Analysis
The chi-squared method was used to analyze the significance of the odor-selective responses made by S. sichuanensis.
The relative electroantennogram (EAG) response value, R, was determined utilizing the following equation: R = (response value of volatile compound - response value of control) / (response value of reference - response value of control). Statistical analysis of the variations in EAG responses among different volatile compounds was performed using the SPSS software package, version 26.0.
Results and Discussion
Cumulative Learning Effects of S. sichuanensis to the Same Stimulus
After experiencing odor source I for three consecutive days, the tropism of 4-day-old S. sichuanensis toward the odor did not improve significantly compared with the tropisms of 4-day-old, 6-day-old, and 8-day-old S. sichuanensis that experienced the mixed odor for one day (Fig. 1, Table 1). Continuous long-term stimulation did not cause significant enhancement of S. sichuanensis behavioral responses to the stimulus; i.e., and there was no obvious cumulative effect of repeated stimulation on learning.
Fig. 1.
Behavioral responses of S. sichuanensis adults to the volatiles of longhorn beetle feces and wood meal after continuous and discontinuous exposures on the second day after eclosion. Volatile I included a mixture of volatiles of the longhorn beetle feces and osier scraps, whereas volatile II included a mixture of volatiles of the longhorn beetle feces and wood meal; this is the same for subsequent figures.
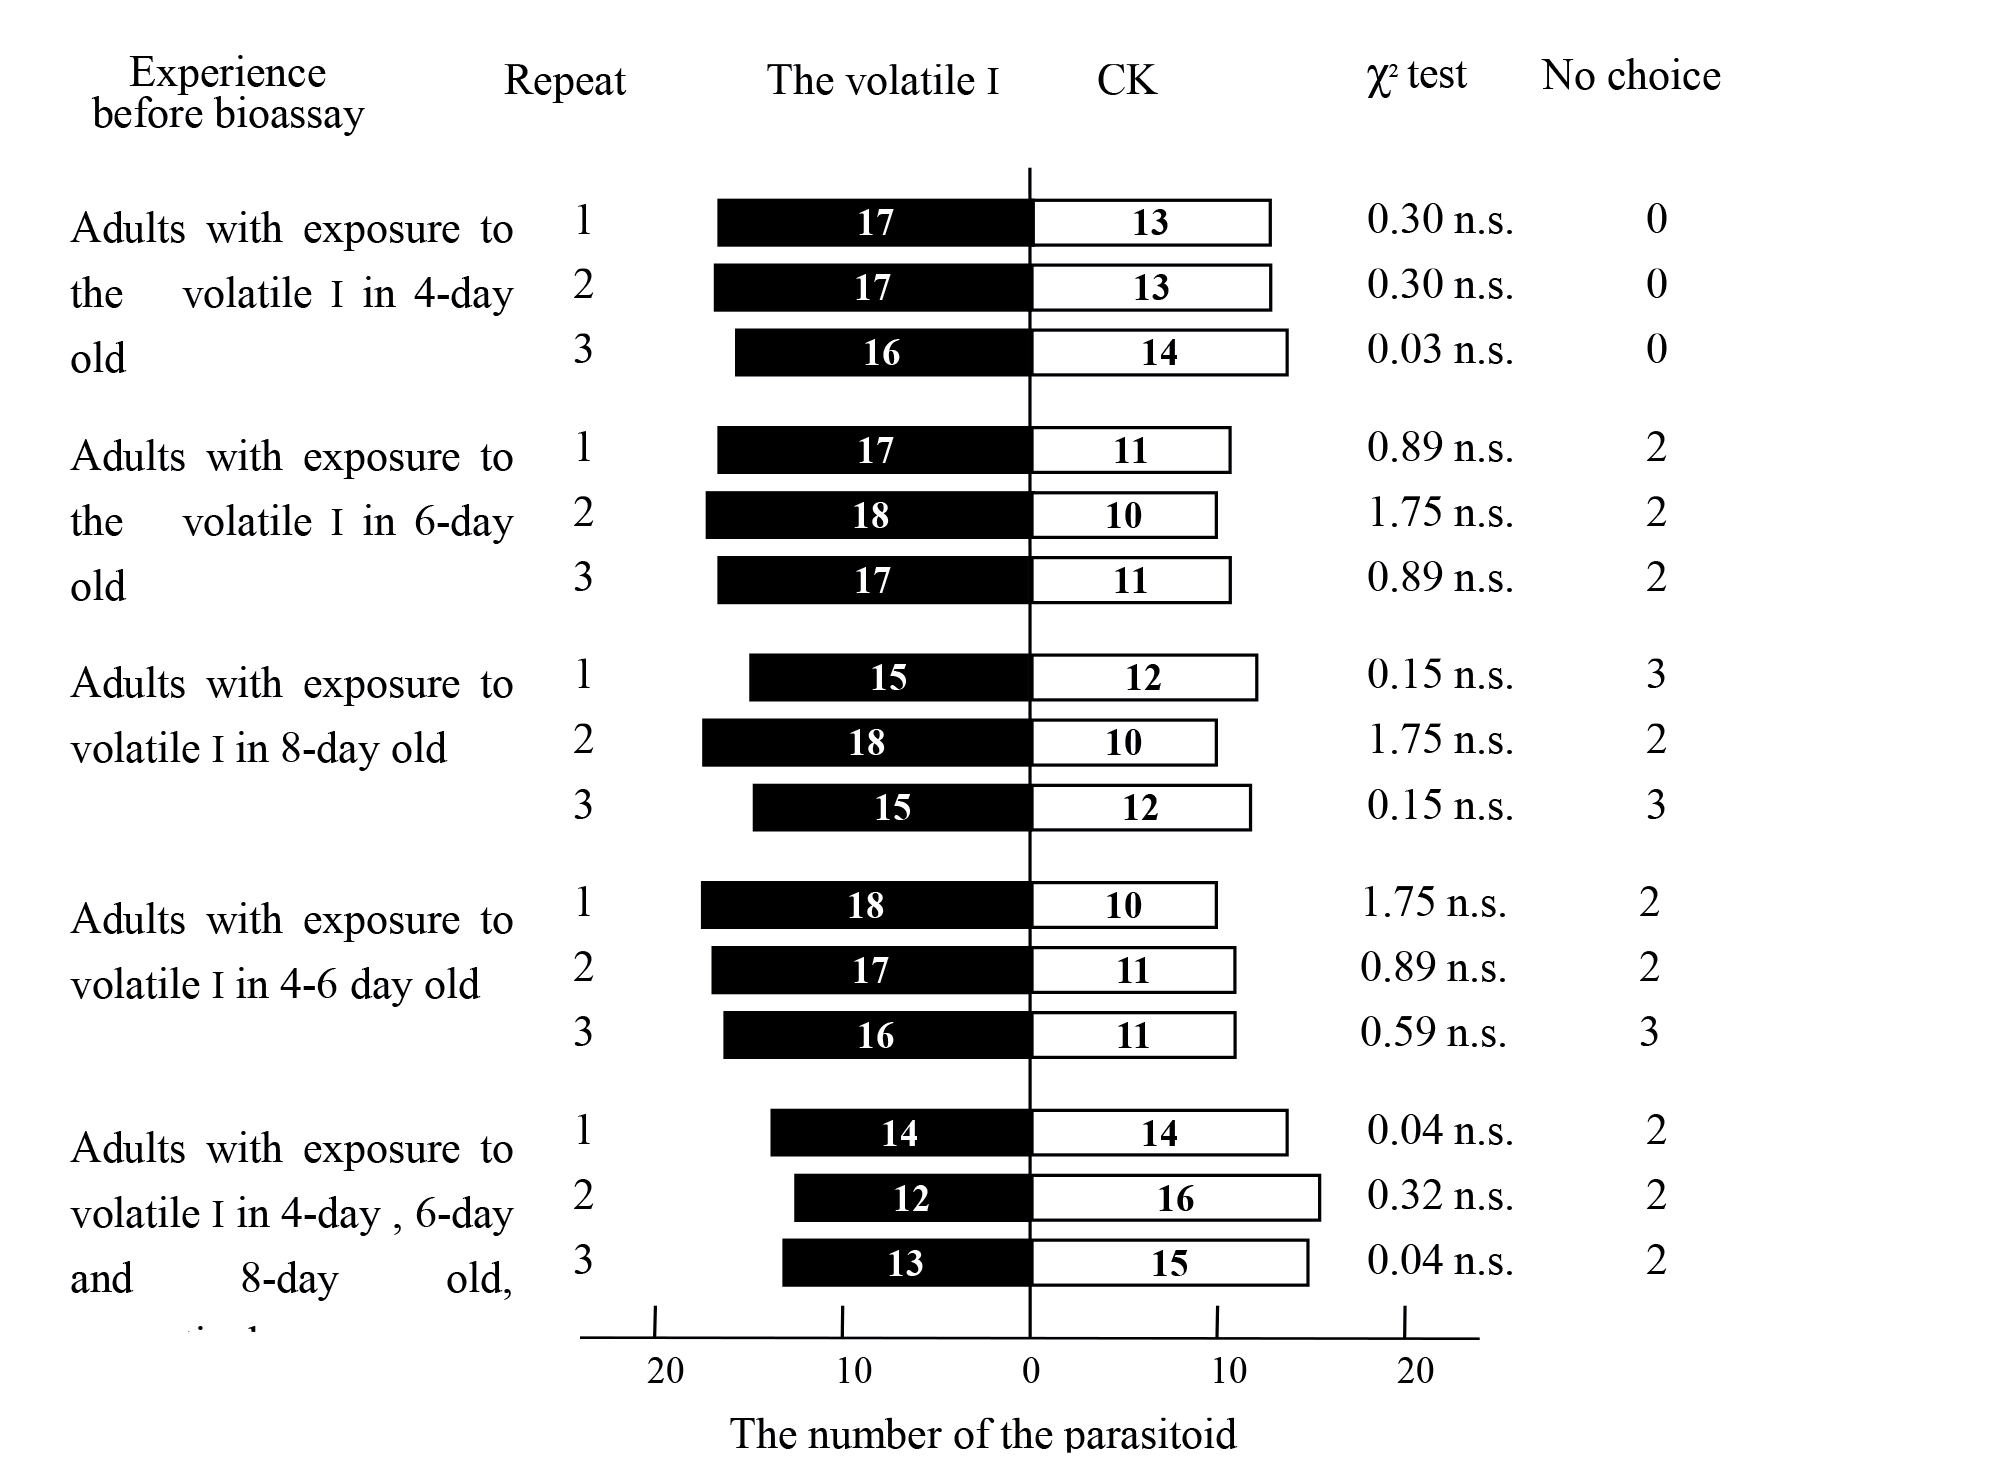
Table 1.
Multiple comparisons for the cumulative learning effect of adults.
After discontinuously repeated exposure to odor source I on the 1st, 3rd, and 5th days, the tropism of 4-day-old S. sichuanensis to the odor was significantly lower than that of 4-day-old, 6-day-old, and 8-day-old parasitoids that experienced the odor source once (Fig. 1 and Table 1). Surprisingly, when S. sichuanensis discontinuously and repeatedly experienced one kind of stimulation, its tropism for this specific stimulation significantly decreased instead of increasing.
Interaction and the Cumulative Effects of Two Different Stimuli on S. sichuanensis Learning
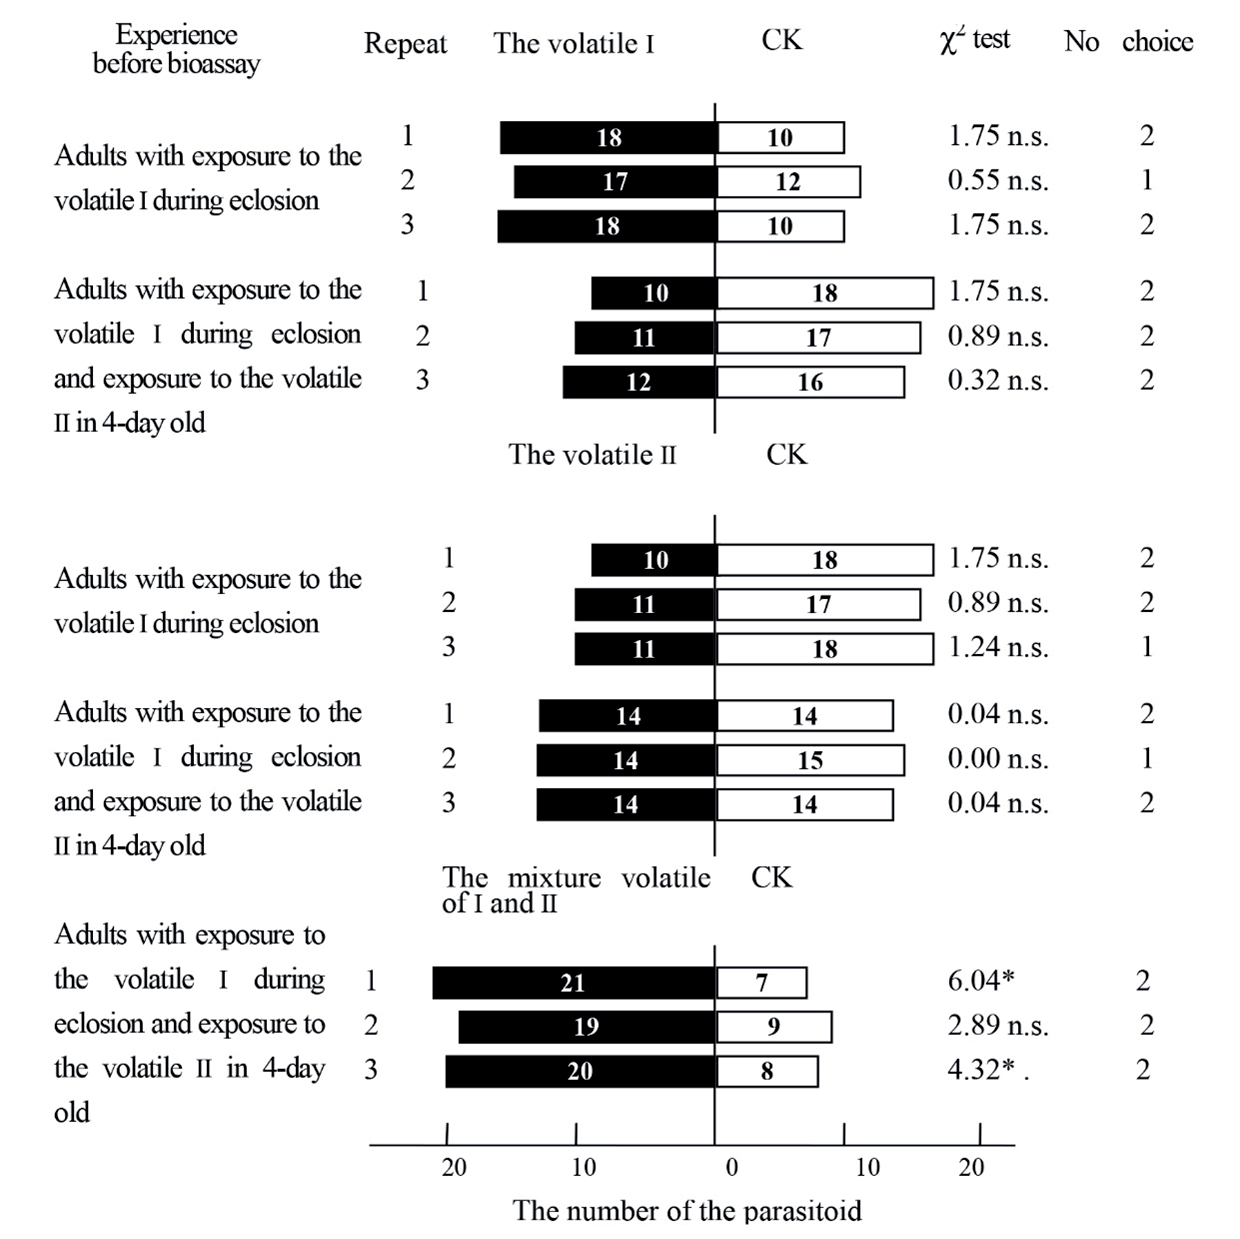
Behavioral response to the stimulating source after experiencing two kinds of stimulation successively: The tropism of the parasitoids to odor source I in treatment 3 was significantly lower than that of adults in treatment 1 (Fig. 2). These tests indicate that the tropism for the first odor decreased, or was “forgotten” after experiencing the second odor. The behavioral response of the adults in treatment 2 to odor source II displayed a certain degree of tropism. The tropism of adults in treatment 4 to odor source II was stronger than that of the adults in treatments 2 and 3, indicating that the behavioral response of S. sichuanensis to the first odor experienced was weakened and a stronger behavioral response occurred toward the second odor after experiencing the second odor. The adults in treatment 5 displayed a stronger tropism to mixed odors I and II at a ratio of 1:1. Two of the three repetitions were significant (Fig. 2). This suggests that different odors experienced by S. sichuanensis can be “superposed,” displaying cumulative effects during learning.
Behavioral responses to the stimulating source after experiencing two kinds of stimulation simultaneously: The selectivity of adults in treatments 7 and 8 to odor sources I and II were equivalent with the average selectivity of 52.38% and 54.76%, respectively (Table 2). Adults in treatment 6 displayed obvious selectivity to mixed odors I and II at a ratio of 1:1. All were significant or highly significant (Fig. 3). This indicates that S. sichuanensis is able to superpose two experienced odors and generate an identification spectrum. The identification spectrum consists of composite volatiles with multiple constituents, and S. sichuanensis was able to identify some constituents of the composite volatiles.
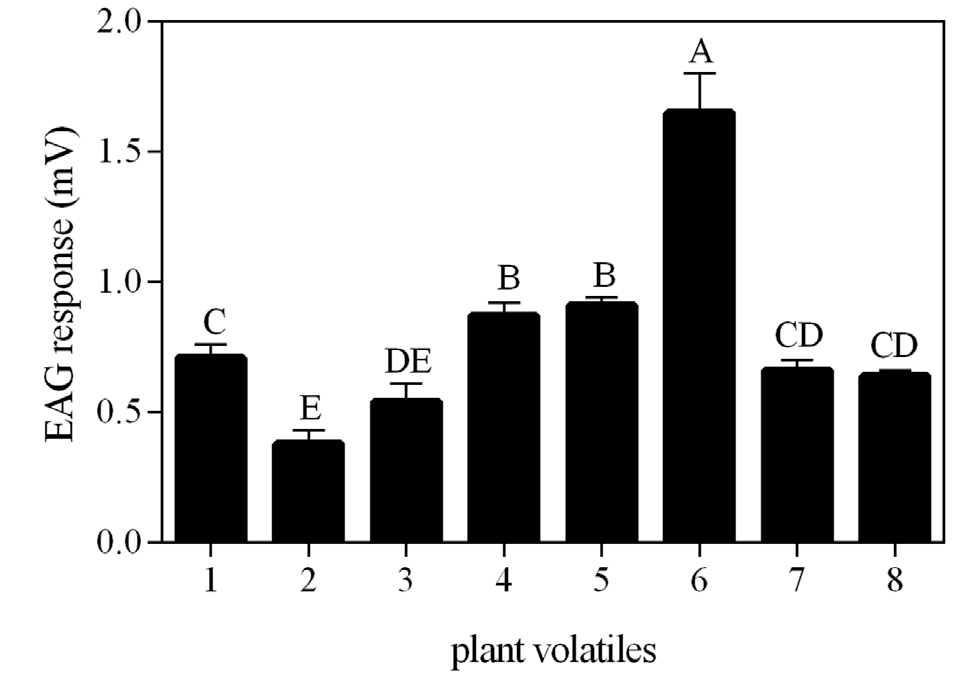
EAG responses of S. sichuanensis adult that experienced odors I and II successively or simultaneously: The EAG response value in treatment 2 was the lowest (Fig. 4). The EAG response value in treatment 6 was the highest followed by treatments 5 and 4. The EAG response value in treatment 6 clearly higher than those in other seven treatments. These results were consistent with the behavioral response results.
Simulated Searching Test of S. sichuanensis
In the laboratory searching test of adults subjected to different treatments (Fig. 5), the average searching time was the shortest in treatment 6 (11.27 s) and the number of successful occurrences was 22 followed by treatment 5 (13.58 s, 18 occurrences). Adults in treatment 2 took the longest time to successfully search for the host (109.60 s, 15 occurrences). The searching time directly reflected the observed learning efficiency of S. sichuanensis, confirming that they exhibit cumulative learning responses.
Effects of Continuously Repeated Experience of the Same Stimulation on Learning by S. sichuanensis
Our behavioral tests showed that the tropism of 4-day-old adults for this mixed odor did not increase after experiencing a mixture of willow and A. chinensis fecula and wood meal for 3 days consecutively. This is consistent with the opinion that parasitoid learning is achieved in a specific and short time period [15].
Habituation is the simplest type of learning behavior in the animal world and refers to the gradual decay of a behavioral reaction during continuous or repeated simulation [16]. The habitual response of insects does not mean acquisition of new responses but refers to repeated contact with some stimulation that decreases the response to that stimulation, and in some cases, specific responses disappear [17, 18]. After repeatedly experiencing the mixture of willow and A. chinensis fecula and wood meal at 4 days old, 6 days old, and 8 days old, instead of increasing, the tropism of these adults to odor decreased significantly compared with that of 4-day-old, 6-day-old, and 8-day-old adults that only experienced the mixture once. This demonstrates S. sichuanensis habituation. During or after the above repeated experience, behavioral responses of S. sichuanensis to the stimulation decreased, presumably because there is no benefit in terms of finding a host or food. An experience that results in no host or food for the parasitoid should cause rapid disappearance of the learning effect [19, 20]. However, habitual responses caused by discontinuous and repeated experience without host or food have not been reported.
Learning Effects of S. sichuanensis that Experience Two Kinds of Stimulation Successively or Simultaneously
After experiencing a mixture of willow and A. chinensis fecula and wood meal on the day of eclosion and then experiencing the mixture of P. orientalis and A. chinensis fecula and wood meal at 4 days old, the selective response to the former decreased significantly (to a level equivalent to that without such experience), and the selective response to the latter was stronger. This phenomenon exists universally in the learning behavior of parasitoids. For example, if female parasitoid Diadegma semiclausum are bred from diamondback moths on Chinese cabbage and then allowed to contact larvae of diamondback moths laying eggs in the cabbage, the selectivity of female D. semiclausum to volatiles released from the diamondback moth–Chinese cabbage complex was higher than that to the volatiles of the diamondback moth–Chinese cabbage composite [21]. This is a significant characteristic of the learning by parasitoids, i.e., behavioral responses caused by learning change in response to a new experience [2].
Table 2.
Duncan’s multiple range results for the behavioral response of adults to two volatiles after experiencing both volatiles.
Fig. 3.
Behavioral responses of S. sichuanensis adults to two volatiles and their mixture after experiencing them simultaneously during eclosion.
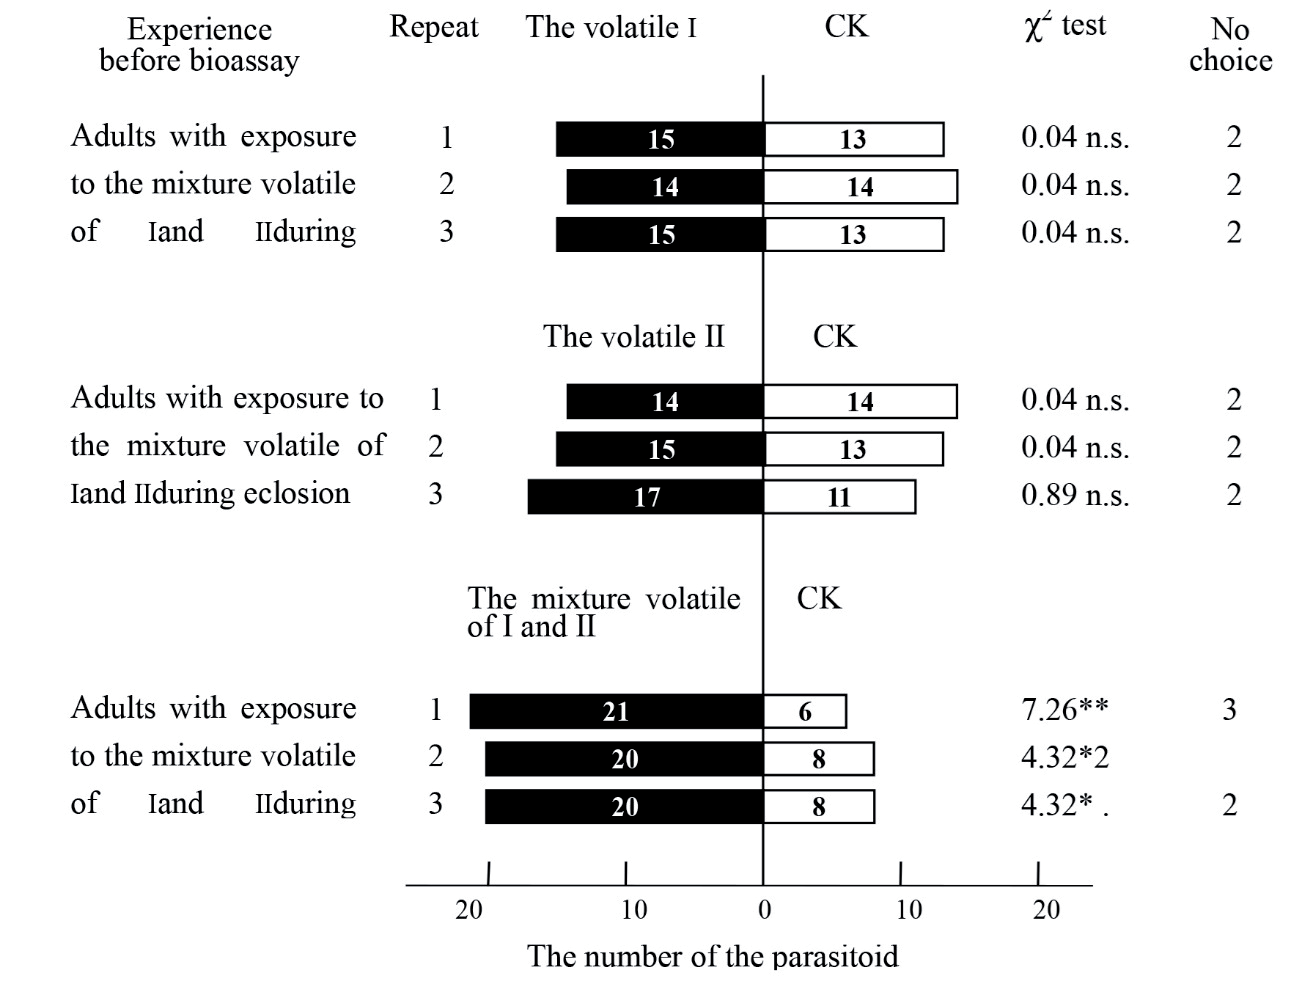
After experiencing joint stimulation by a mixture of A. chinensis fecula and wood meal from two types of trees, on the eclosion day and during the early adult stage, S. sichuanensis showed obvious behavioral responses to separate stimulation by the two substances at 4 days old. However, the selectivity of the response was significantly lower than in those that experienced only one of the two substances. During associative learning, two kinds of simultaneous stimulation can be experienced by parasitoids: non-conditioned stimulation and conditioned stimulation [22]. Our tests allowed S. sichuanensis to experience two stimuli and then mixtures of the two kinds of stimulation. Adult S. sichuanensis certainly had the ability to recognize the components of the stimulus mixture.
This phenomenon was firstly discovered in this study. After experiencing stimulation by two information substances, successively or simultaneously, parasitoids showed strong behavioral responses to the mixture. After experiencing mixed stimulation by A. chinensis fecula and wood meal on two kinds of trees on the eclosion day and during the early adult stage, 4-day-old S. sichuanensis selectivity of the mixed odor was high. After experiencing the mixture of willow and A. chinensis fecula and wood meal on the eclosion date and during the early adult stage, they experienced P. orientalis and A. chinensis fecula and wood meal at 4 days old. These tests demonstrated that learning behavior of S. sichuanensis is cumulative because they can integrate two kinds of chemical information experienced simultaneously and recognize the two odors experienced successively. Further study was required to explore whether these learning effects are universal among parasitoids and their mechanisms.
Fig. 4.
The synergized EAG response of the adults to two volatiles after previously experiencing them. Numbers under the abscissa refer to the treatment numbers in the main text. Values with the same letter labels are not significantly different from each other.
Associative learning by parasitoids has been reported in Microplitis croceipes, Cotesia kariyai, Diachasmimorpha kraussii, Ascogaster reticulata, Psyttalia concolor and other hymenopteran insects [3, 6, 23-25]. The present study revealed two novel learning behaviors in a parasitoid: habitual responses and cumulative effects. These findings provide a breakthrough in elucidation of learned behavioral mechanisms in parasitoids and will help in the development and application of using natural enemy insects for pest control.
Conclusions
This study unveils a novel phenomenon, where parasitoids exhibit strong behavioral responses to the mixture of two information substances after being stimulated by them successively or simultaneously. Two distinct learning behaviors, habitual responses and cumulative effects, have been discovered in S. sichuanensis. Notably, these parasitoids can integrate two chemical information sources experienced simultaneously, as well as superimpose two sequential odor cues for identification purposes. These findings represent a significant breakthrough in understanding the learning-behavioral mechanisms of parasitoids and have important implications for the development and application of natural enemy insects in pest control strategies.

