

Introduction
Soil extracellular enzymes are proteins with a specific catalytic capacity secreted by soil microorganisms and other organic tissues (such as soil fauna, plant roots, and sand residues) and play a critical role in regulating nutrient cycling and fixation in soil system [1, 2]. Numerous studies show that four soil extracellular enzymes (β-1,4-glucosidase, BG; β-1,4-N-acetylglucosaminidase, NAG; L-leucine aminopeptidase, LAP; acid phosphate, AP) are involved in the C, N, and P cycles of soil microorganisms [3-5]. The ratios of BG, NAG + LAP and AP can be used to calculate the soil extracellular enzyme stoichiometry. These ratios represent the relative abundance of C-, N-, and P-acquiring enzymes [3, 5] and reflect the nutritional needs of microorganisms and the nutrition supply in the soil [2, 6]. Therefore, the study of soil enzymatic stoichiometry is fundamental to understanding nutrient turnover, cycling and balance in soil systems and has become a research hotspot in the past decade [7, 8].
Both biotic and abiotic factors impact soil extracellular enzyme activities (EEAs) and their stoichiometric ratios at different spatiotemporal scales and ecosystems, such as stand age, soil quality, and ecosystem stress [2, 8]. Brockett et al. [9] report a significantly negative relationship between soil moisture content and soil EEAs in a forest ecosystem. Another study shows that the relationship between soil nutrients and pH limits soil EEAs in a tundra ecosystem [10]. A similar study also shows most changes in soil EEAs are determined by soil C and N contents [11]. The proportion of microorganism acquisition in tropical forests is affected by climatic conditions, vegetation types, and soil geochemistry [12, 13]. Results from these studies suggests the driving factors regulating variation of soil EEAs may be enzyme specific or ecosystem specific, and therefore, understanding for the underlying mechanisms in soil EEAs variation and stoichiometry are still limited.
Stand age can impact litter accumulation, root exudates, and the soil microenvironment (water content, pH, effective nutrient content), resulting in changes in the structure and composition of microorganisms, thus affecting soil EEAs [14]. A recent study shows oxidative enzyme activity decreases with stand age, while no significant change is found in the hydrolytic enzyme activity [15]. However, another study found hydrolytic enzyme activity increases with stand age [16]. Furthermore, Qiao et al. [17] reported soil EEAs (i.e., BG, α-cellulases, NAG, LAP, and AP) increase with increasing stand age along a chronosequence of Camellia oleifera plantations. Dong et al. [18] indicates the soil enzymatic C:N ratio is positively correlated with stand age, while the soil enzymatic N:P ratio is negatively correlated with stand age in Pinus massoniana plantations. How the stand age of plantations affects soil EEAs and stoichiometric ratios requires further exploration.
Illicium verum (Magnoliaceae), also known as star anise, is an important economic tree species broadly planted in the mountainous areas in tropical and subtropical regions of southern China including Guangxi, Guangdong, Fujian, and Yunnan Provinces [19]. The fruit from I. verum is widely used as a cooking ingredient and in important traditional Chinese medicine for treating rheumatism, stomachache, and insomnia [20]. The fruit, branch, bark, and leaf are rich in fennel oil, which has antioxidant, antiviral and antibacterial properties [21]. Guangxi Province is the origin and main production area of I. verum, and the star anise yield accounts for nearly 90% of total annual production in China [22, 23]. However, the yield of star anise per unit area is generally unstable and low because of improper plantation management in Guangxi, which hinders sustainable development in the star anise industry of China [19, 23].
Most studies have focused on the traditional use, phytochemistry, pharmacology and toxicology of star anise [20, 21, 24]. Less attention has been given towards exploring planting and management measures, especially the effects of soil biological and physicochemical properties on planting quality and yield. A previous study shows soil nutrients are low in Gauanxi’s I. verum plantations [25]. Moreover, a recent study indicates that the associations between nutrient links, soil microbial properties, and the detritus food web govern ecosystem functioning in I. verum plantations [19]. The development of plantations inevitably causes differences in nutrient availability for soil microorganisms among stands with different ages, therefore affecting the limiting factors of soil microbial nutrients. However, there are no studies on soil EEAs and stoichiometry along an I. verum plantation chronosequence in southern China, and the major limiting factors of microbial nutrients in the plantations are still unclear.
In this study, we analyze soil physicochemical properties, soil EEAs, and enzymatic stoichiometry in I. verum plantations, among different stand ages, in a tropical mountainous area of southern China. We hypothesized that (1) soil EEAs increase with stand age and soil physicochemical properties would affect the soil EEAs and stoichiometry, and (2) microorganisms would be limited by P in the I. verum plantations. Our aim is to promote the sustainable use of soil resources and enhance the management strategies of I. verum plantations in southern China.
Materials and Methods
Study Area
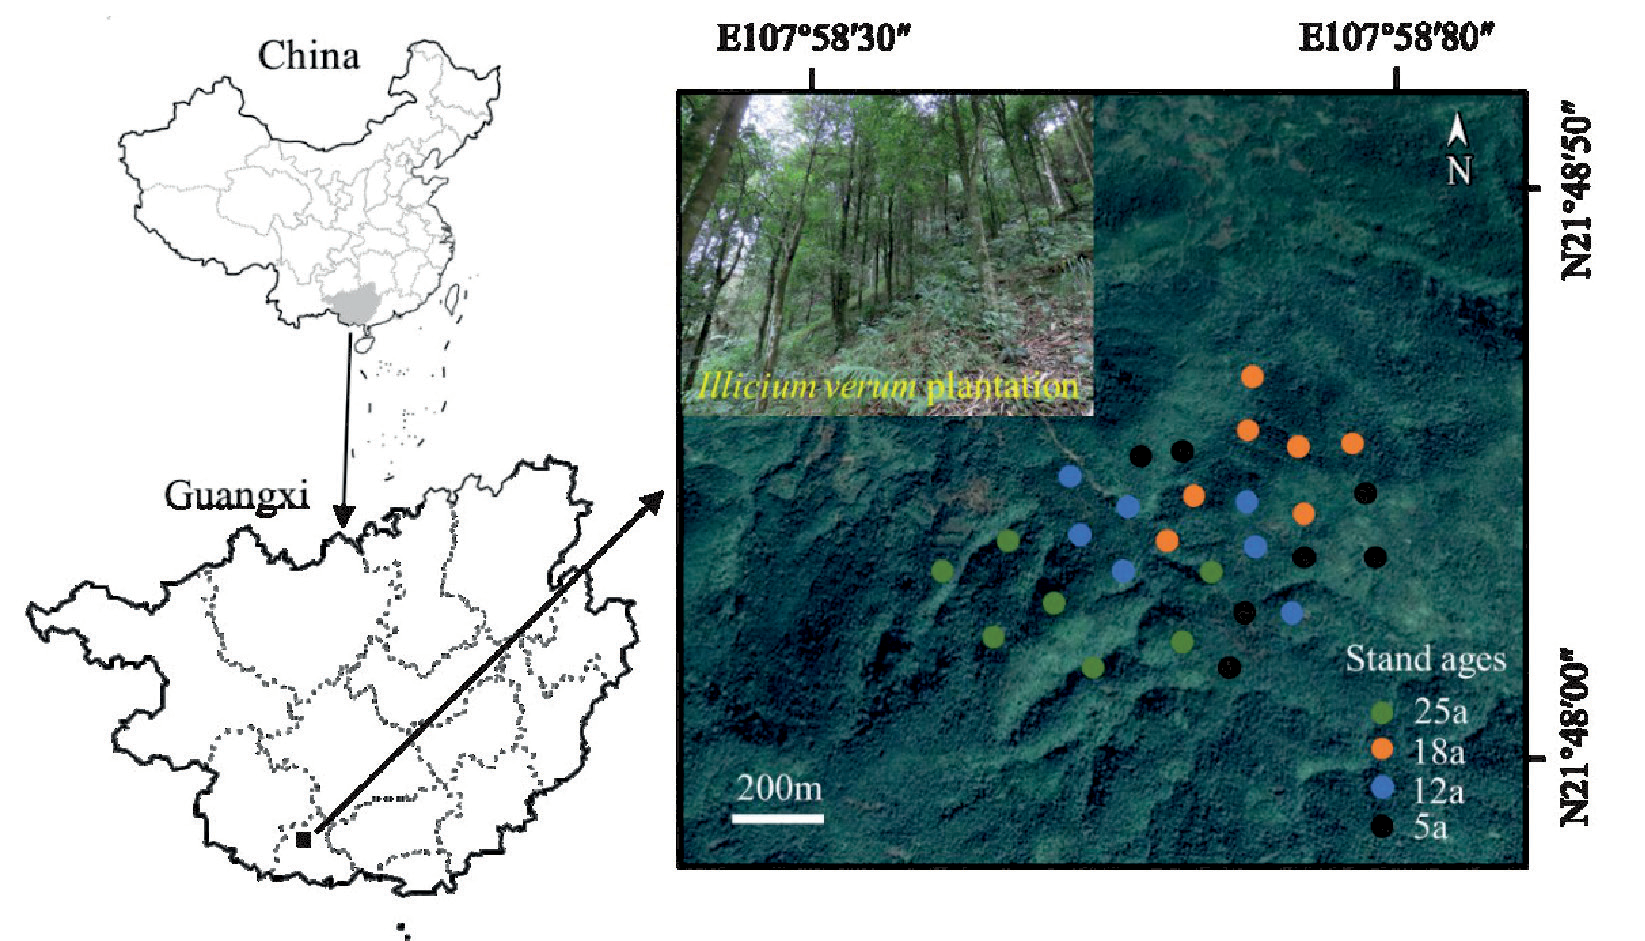
The study area is located in a mountainous area (E107º58′50″, N21º48′25″) in Fangchenggang City, Guangxi Province, southern China, at an elevation of 350-670 m (Fig. 1). The study site is in a tropical monsoon climate area. The annual sunshine is 1525 h, the average annual temperature is 21.9ºC, and the average annual rainfall is greater than 2900 mm. The soil type is an acid lateritic red soil. The common understory plants in the I. verum plantations include: Paeonia delavayi, Maesa japonica, Melicope pteleifolia, Arthraxon hispidus, Dicranopteris pedate, and Oplismenus undulatifolius. The study area is one of the main production areas of star anise in Guangxi Province. This I. verum plantation covers nearly 7000 ha with an annual yield of 6000 t dry fruits of star anise.
Soil Sampling
Soils were sampled in July of 2021, during peak growing season. Four stand ages (5a, 12a, 18a, and 25a) of I. verum plantations were selected. Seven plots (each 20 × 20 m) were set up for each stand age (Fig. 1). Surface soil (0-20cm) was collected with a 10 cm diameter auger after removing the litter, roots and gravel. Five soil samples were collected along an S-shaped curve within each plot and then mixed together. The fresh soil samples were first placed in 4ºC ice boxes in the field and then kept in a 4ºC refrigerator in the laboratory. Some soil samples were used to determine water content and extracellular enzymes, and the rest were air-dried to measure soil properties. The site properties and stand characteristics of I. verum plantations are presented in Table 1.
Measurement of Soil Properties and EEAs
The pH of air-dried soil samples was determined by PHS-3C pH meter (Leici Instruments Co., Shanghai, China). The soil water content (SWC) was measured using standard gravimetric method. SOC was determined by the H2SO4-K2Cr2O7 oxidation method. STN was measured via the Kjeldahl method. STP was measured colorimetrically after wet digestion of samples with H2SO4+HClO4. SAN was analyzed with the microdiffusion technique after samples were subjected to alkaline hydrolysis. SAP was analyzed by the Olsen method. All methods were used for determining soil physicochemical properties as described by Lu [26].
The four soil EEAs were measured using the methods of Peng & Wang [27]. 4-MUB-β-D-glucopyranoside, 4-MUB-N-acetyl-β-D-glucosaminide, L-leucine-7- amino-4-methylcoumarin, and 4-MUB-phosphate were selected as fluorometric substrates of BG, NAG, LAP, and AP, respectively. 1 g of fresh soil stored at –4ºC was weighed into a beaker, 125 mL of acetic acid buffer (50 mmol/L, pH 5.0) was added, and the mixture was mixed with a vortex oscillator to prepare a soil suspension. Next, 200 μL of soil suspension was added to each well of a 96-well microplate, and 50 μL of substrate (200 μmol/L, prepared with ultrapure water) was added. All microplates were incubated in the dark at 20ºC for 4 h, and then 10 μL of NaOH solution (1 mol/L) was added to each well to terminate the culture. After one minute, a multifunctional microplate reader (Synergy H4, BioTek, Winooski, USA) was used for excitation at 365 nm and fluorescence measurement at 450 nm.
Table 1.
Site properties and stand characteristics of Illicium verum plantations with four stand ages. Values are the mean±standard error.
Data Analysis
One-way ANOVA was used to test the significance between stand ages (LSD, α = 0.05). When necessary, data was logarithmically (log) transformed to meet the assumption of normality and homoscedasticity. Pearson analysis was then applied to determine the relationships of soil EEAs, enzyme stoichiometric ratios and soil physicochemical properties according to the significance level using SPSS 26.0 (IBM-SPSS Inc., Chicago, USA). Redundancy analysis (RDA) is a well-known multivariate statistical technique that commonly used to explore and explain the relationships among multiple variables [28]. The associations between soil EEAs, enzyme stoichiometric ratios, and soil physicochemical properties were examined by RDA, performed using CANOCO 4.5 [28].
Results and Discussion
Changes in Soil Properties, Soil EEAs and Stoichiometry in I. verum Plantations
As shown in Table 2, the soil from the I. verum plantations was acidic (4.57±0.18). Soil pH decreased with increasing stand age. The soil pH values at 18 a and 25 a were significantly lower than 5 a and 12 a (p<0.05). SWC increased with increasing stand age. Stands at 18 a and 25 a were significantly higher than 5 a and 12 a (p<0.05). The SOC, STN, soil N:P ratio (SNP), soil C:P ratio (SCP), soil C:N ratio (SCN), and SAN significantly increased with increasing stand age (p<0.05), while the STP and SAP did not significantly change with stand age (Table 2).
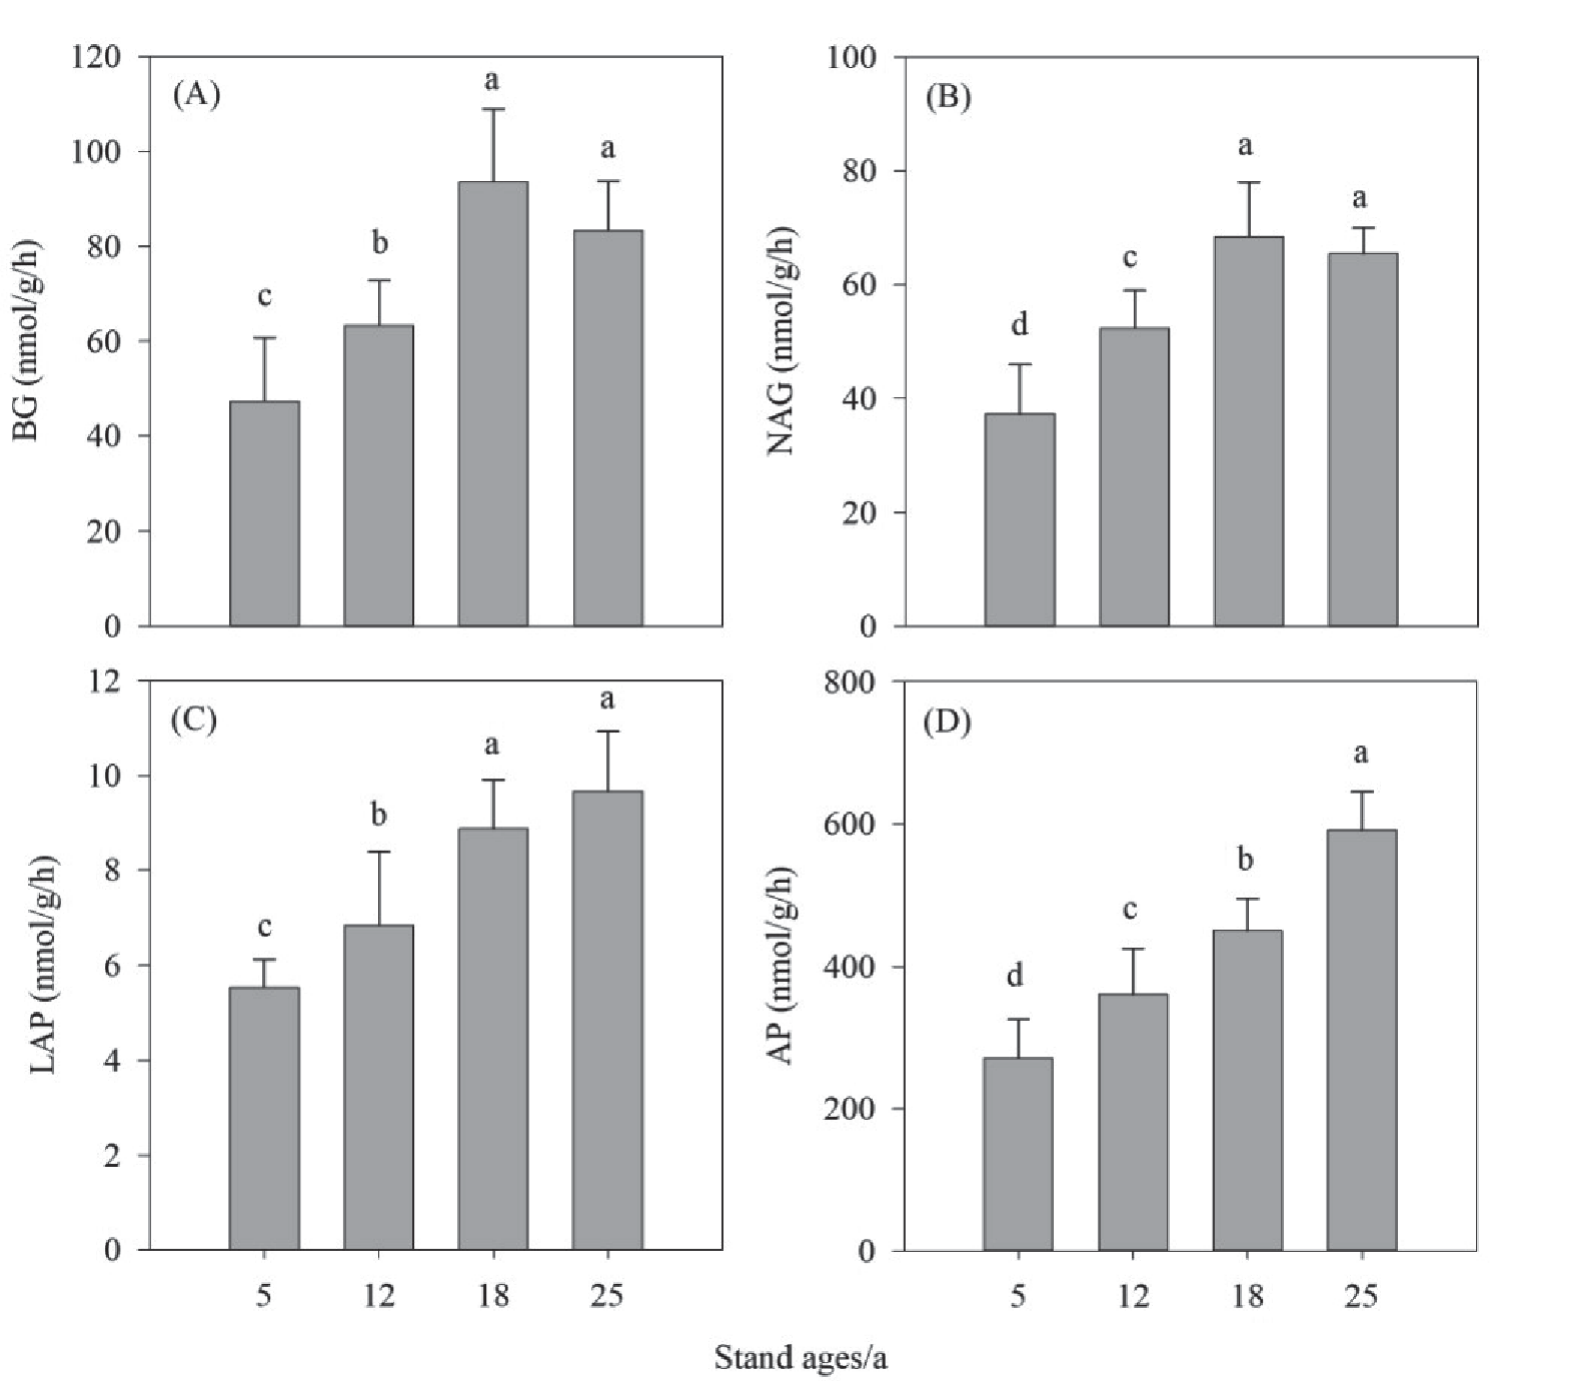
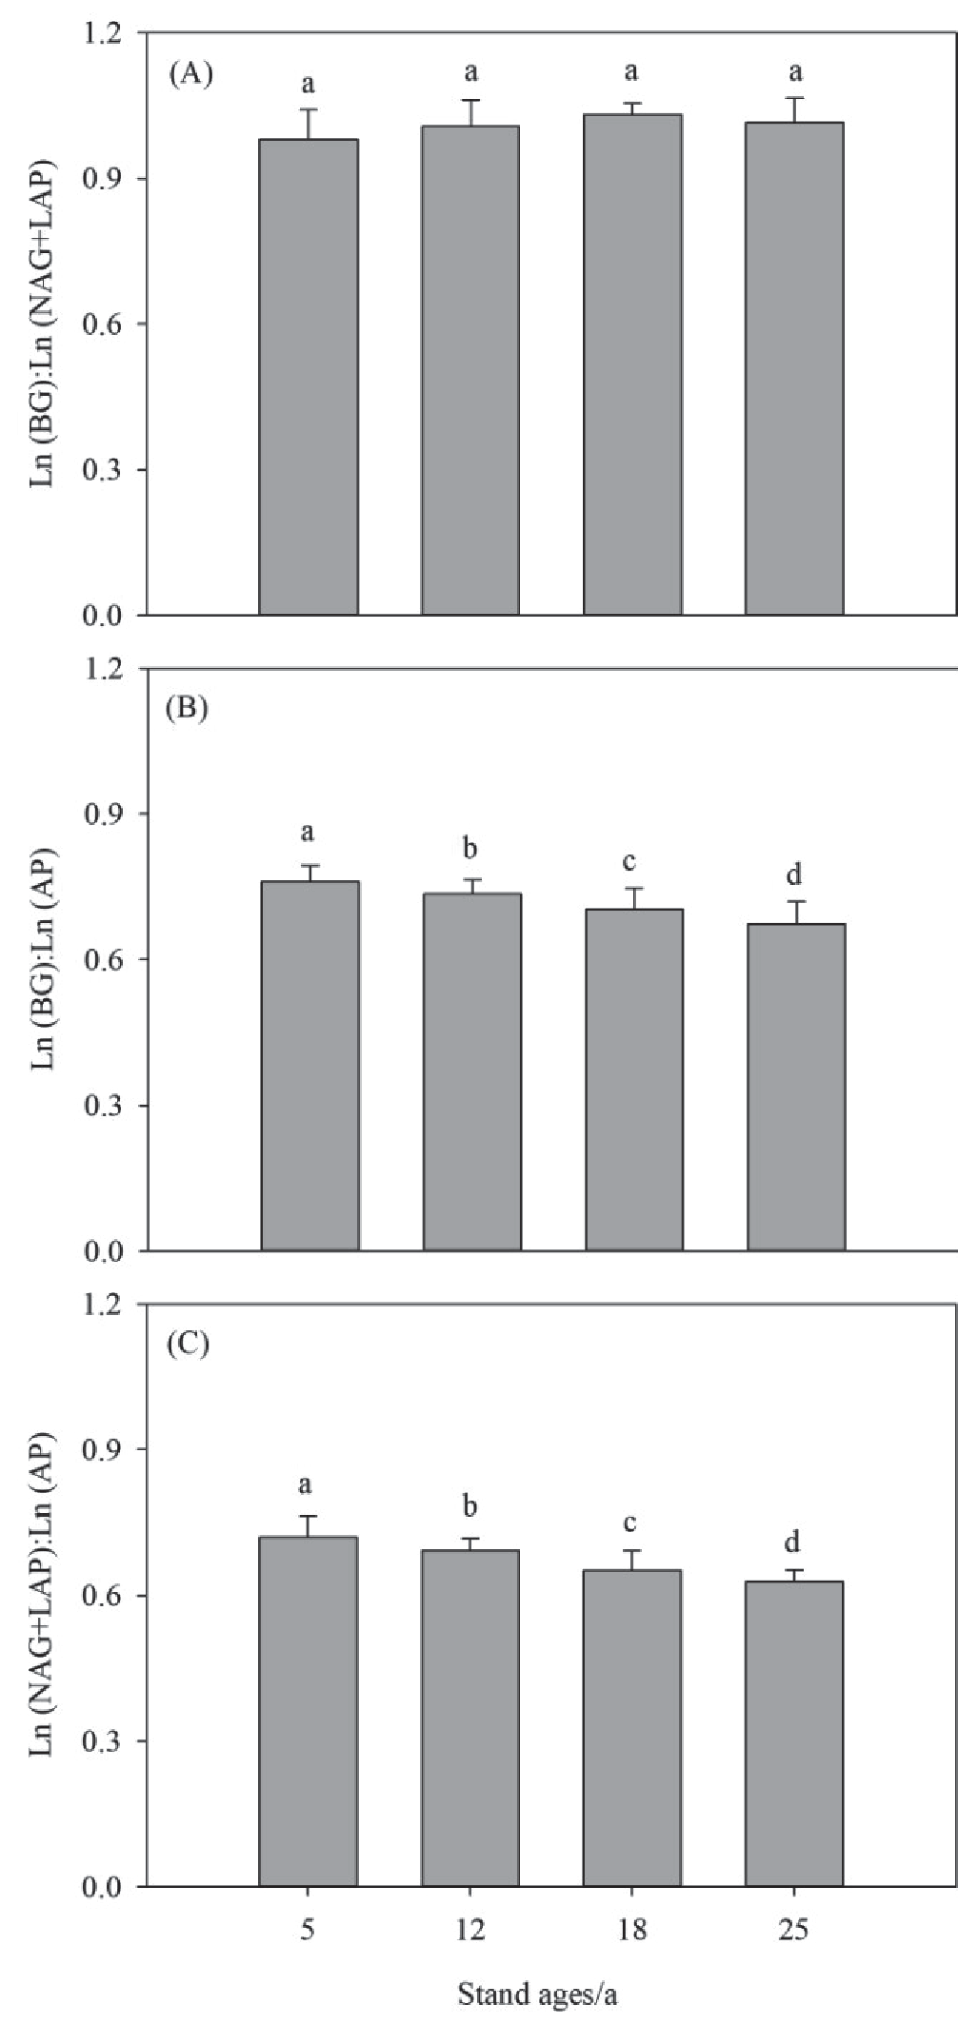
The changes in the four EEAs showed an increasing trend as stand age increased (Fig. 2). There was no significant difference in the BG activity between the 18 a and 25 a stands, but they were significantly higher than the 5 a and 12 a stands (p<0.05) (Fig. 2a). NAG activity significantly increased from the 5 a to 18 a stands (p<0.05) but decreased slightly in the 25 a stands (p>0.05) (Fig. 2b). LAP activity increased with increasing stand age, but there was no significant difference between 18 a and 25 a (p>0.05) (Fig. 2c). AP activity increased significantly with increasing stand age (p<0.05) (Fig. 2d). The soil enzymatic C:N:P ratio was 1:1:1.4. The soil ECN showed no significant difference among the four stand ages (Fig. 3a), while both soil ECP and ENP significantly decreased with increasing stand age (p<0.05) (Fig. 3(b-c).
Table 2.
Soil physicochemical properties in Illicium verum plantations with four stand ages.
[i] pH – soil pH; SWC – soil water content; SOC – soil organic carbon; STN – soil total nitrogen; STP – soil total phosphorus; SCN – soil C:N; SCP – soil C:P; SNP – soil N:P; SAN – soil available nitrogen; SAP – soil available phosphorus. Different lowercase letters indicate significant differences among different stand ages (p<0.05). Values are presented as the means±standard errors (n = 7).
This study shows STN, SAN, SOC, SCN, SCP, and SNP and four EEAs increased with stand age (Table 2, Fig. 2) and relates to the litter yield, decomposition rate, and root biomass in I. verum plantations at different stand ages. The young I. verum plantations (5 a) have a fast growth rate, requiring sufficient soil nutrients to meet growth needs and compete with soil microorganisms for N and P nutrients. Therefore, this is likely the reason the soil nutrients and EEAs were lower. However, in the mature plantations (18 a and 25 a), the growth of I. verum is relatively slow, the soil nutrient accumulation rate is lower, and the soil EEAs increases gradually and tends to be relatively stable. The understory litter and plant residues increase with stand age, enhancing the contents of SOC and STN. In addition, with the increase in stand age, the enhanced soil biological activity promotes the decomposition and transformation of soil organic matter, thereby further facilitating the release of C and N. Moreover, the growth and development of the root system of I. verum may contributes to the reduction of soil erosion, thus leading to a decrease in the loss of soil C and N. Therefore, which provides C and N sources for soil microorganisms to grow, and further enhances the soil EEAs [29]. Some studies show soil EEAs are significantly higher in soils with vegetation with more root biomass [30, 31]. Therefore, I. verum plantations develop more fine roots with increasing stand age, which can produce more soil extracellular enzymes by releasing exudates [32]. In addition, long-term soil microbial C fixation, N fixation and atmospheric N deposition also led to the accumulation of soil nutrients with increasing stand age, thereby enhancing the soil EEAs.
The soil was red soil with a high content of iron and aluminum ions in the study area, thus P is easily complexed into forms that are more inaccessible to plants and microorganisms, resulting in serious soil P limitation [12]. Moreover, abundant rainfall and leaching further decreases the soil P availability [33]. Therefore, STP and SAP are low in I. verum plantations. Previous studies have also shown SAP in I. verum plantations within Guangxi ranges from 0.8 to 1.5 mg/kg, and P is severely deficient in the study area [25]. Notably, AP activity increases with stand age (Fig. 2), which is related to the soil P deficiency in the study area. In conclusion, the soil EEAs increase with the age of I. verum plantations, supporting our first hypothesis.
Factors Influencing the Soil EEAs and Stoichiometry in I. verum Plantations
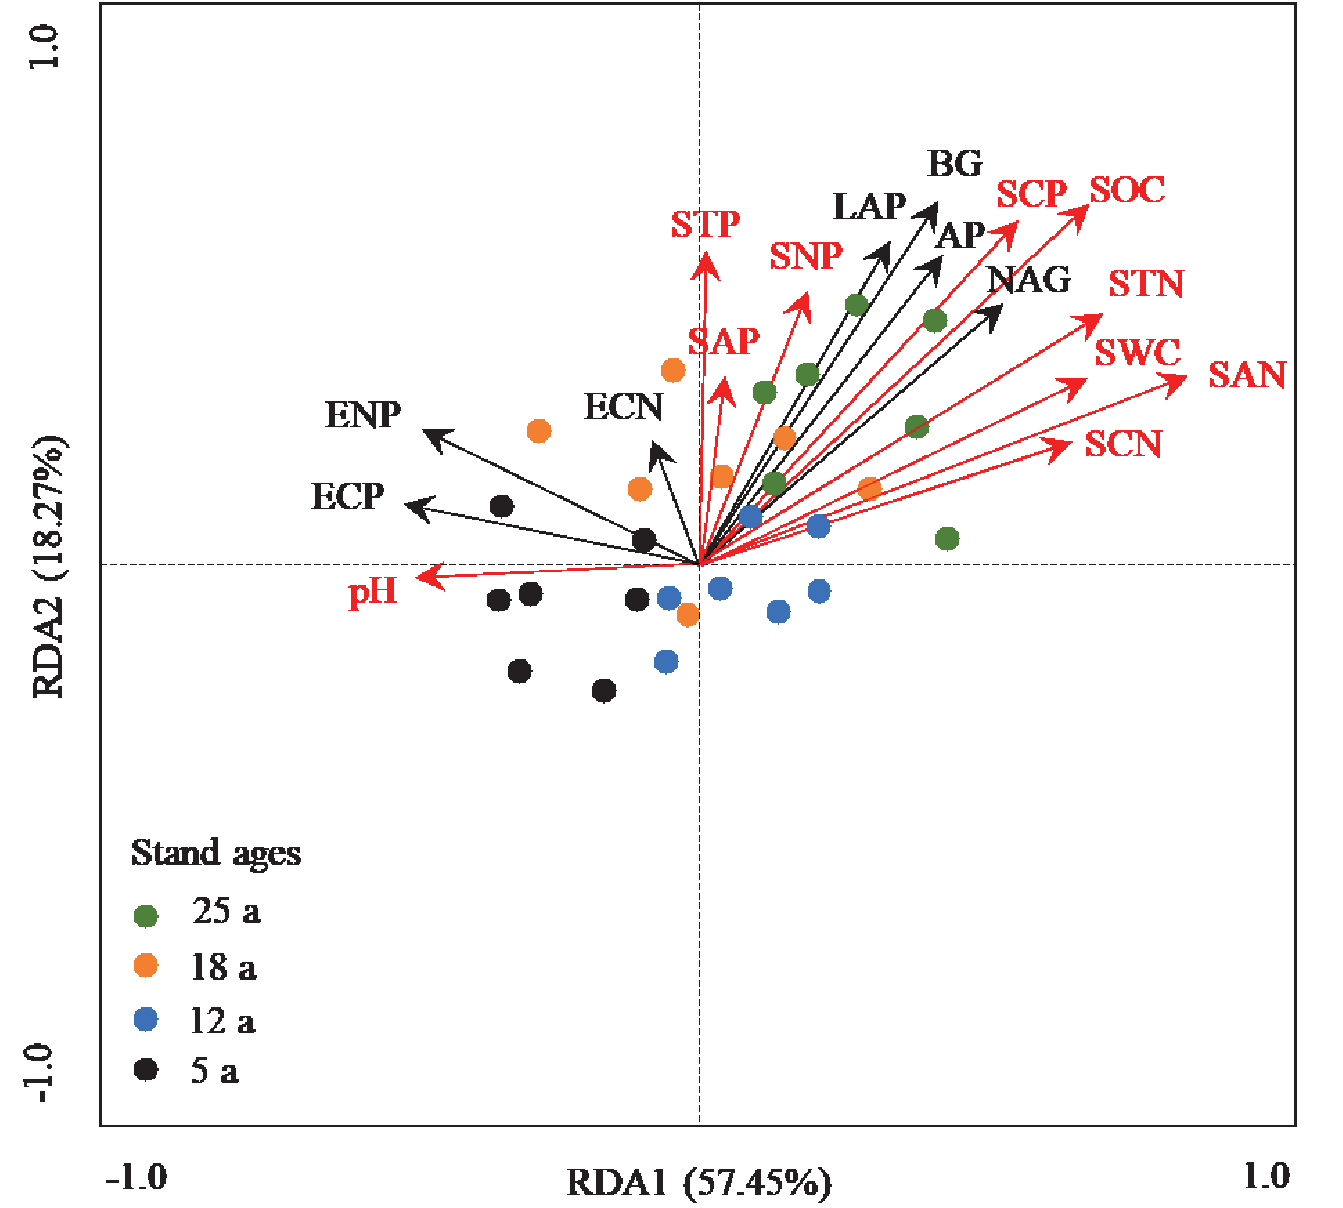
As shown in Table 3, soil pH and the activities of NAG and AP (p<0.05) were significantly and negatively correlated. SWC and SOC had significantly positive correlations with the four EEAs and their ratios (p<0.05) (Table 3). STN and SAN showed a significant positive correlation with the four soil EEAs, while STP, SAN and SAP showed a significant negative correlation with ECP and ENP (p<0.05). The RDA results showed that the explanatory variables of the first axis and the second axis were 57.45% and 18.27%, respectively (Fig. 4). SWC, SOC, SCN, SCP, SNP, BG, NAG, LAP, AP, and ECN showed significantly positive correlations with each other and negative correlations with soil pH, ECP and ENP (p<0.05) (Fig. 4).
Many studies report abiotic factors have a significant impact on soil EEAs and that the contribution rate is greater than biotic factors [34]. In a synthesis of 40 studies, soil EEAs are found to be largely influenced by the soil pH, soil organic matter, and climate factors [35]. Soil EEAs and their stoichiometry are affected directly by SWC and soil pH and indirectly by SOC, STN, and SAN [8, 36]. Our study shows SWC is positively correlated with four soil EEAs in I. verum plantations (Table 3, Fig. 4), which is consistent with the findings of previous studies [35]. A higher SWC can accelerate root growth and similarly enhance the activity of microorganisms [37], directly enhancing the ability of plants and microorganisms to secrete extracellular enzymes [38]. A high SWC contributes to leaching of nutrient elements in soil and accelerates the absorption of soil nutrients by plants. This results in a decrease of soil nutrient availability [39], thus increasing the nutrient demand of microorganisms and indirectly affecting the soil EEAs. pH is a critical soil property affecting soil EEAs and stoichiometry [35, 40]. A low soil pH enhances the geochemical adsorption of P and prevents P from migrating through the soil [3], leading to a decrease in P availability in I. verum plantations.
The contents of soil nutrients can greatly affect soil EEAs and their stoichiometric ratios by affecting soil available substrate and soil C:N:P stoichiometric characteristics [34]. The correlation analysis shows soil ECP and ENP have a significantly positive correlation with SOC (Table 3). The high ECP and ENP in soil indicates SOC content increased, which simultaneously promotes the secretion of extracellular enzymes by soil microorganisms. Therefore, SOC is an important factor affecting the soil EEAs and enzymatic stoichiometry in I. verum plantations. Our results are consistent with previous studies, showing soil nutrition and stoichiometry have great effects on soil EEAs and enzymatic stoichiometry [10, 37]. Overall, the SWC, soil nutrients, and soil C:N:P stoichiometry are identified as the major soil variables affecting soil EEAs and enzymatic stoichiometry in I. verum plantations, which is consistent with our first hypothesis.
Soil P Limitation in I. verum Plantations
The extracellular enzyme stoichiometry represents a biogeochemical balance between substrate availability and microbial resource allocation in soil system [41, 42]. Sinsabaugh et al. [35] reported that the stoichiometric ratios of soil EEAs are 1:1:1 in the global ecosystem. Consequently, the supply rates of assimilable substrates of C, N, and P are often quantitatively similar, demonstrating the stoichiometric homeostasis of soil microorganisms [2, 3]. However, there are significant differences in soil enzyme stoichiometry owing to substrate availability, as well as biotic and abiotic factors [43]. In the present study, the ratio of soil C-, N-, and P-acquiring enzyme activity in I. verum plantations is 1:1:1.4, which deviates from 1:1:1 at the global scale. This indicates the study area has a high activity of P-acquiring enzymes, reflecting the relative lack of P in soil. As stands increase in age, the soil P-acquiring enzyme activity increases significantly, while the soil ECP and ENP decrease significantly (Fig. 2 and 3). This indicates microorganisms become more restricted by P with increasing stand age, verifying our second hypothesis.
Table 3.
Correlations between soil enzyme activities, enzymatic stoichiometry, and soil physicochemical properties.
[i] ECN – ln(BG):ln(LAP + NAG); ECP – ln(BG): ln(AP); ENP – ln(LAP + NAG):ln(AP); pH – soil pH; SWC – soil water content; SOC – soil organic carbon; STN – soil total nitrogen; STP – soil total phosphorus; SCN – soil C:N; SCP – soil C:P; SNP – soil N:P; SAN – soil available nitrogen; SAP – soil available phosphorus. * p<0.05; ** p<0.01. BG, NAG, LAP, and AP indicate β-1,4-glucosidase, β-1,4-N-acetylglucosaminidase, leucine aminopeptidase, and acid phosphatase, respectively.
Resource allocation theory suggests soil microorganisms can produce extracellular enzymes by consuming abundant elements to mine relatively limited elements [44, 45]. The high demand for P of the microorganisms reflects the deficiency of elemental P. The P concentration in soil is determined mainly by the weathering of minerals and is gradually consumed by plant growth during stand development [2]. The increased input of plant residues led to a decrease in soil pH with plantation time (Table 2), while the migration of P was limited by lower pH in the soil system [46]. In response to the increase in C and N and the decrease in P in soil during stand development, soil microorganisms can gradually enhance the expression of AP enzyme, resulting in lower ratios in soil ECP and ENP with stand age (Fig. 3). Our results are consistent with most studies that consider P in the tropics to be the limiting factor for ecosystem productivity [12, 47, 48]. Therefore, more attention should be given to the input of P elements in the management of I. verum plantations.
Fig. 4.
Ordination plots of redundancy analysis to identify the relationships among the soil enzyme activities, enzymatic stoichiometry, and soil physicochemical properties in four stand ages (5 a, 12 a, 18 a, and 25 a). ECN – ln(BG):ln(LAP + NAG); ECP – ln(BG): ln(AP), ENP – ln(LAP + NAG):ln(AP); pH – soil pH; SWC – soil water content; SOC – soil organic carbon; STN – soil total nitrogen; STP – soil total phosphorus; SCN – soil C:N; SCP – soil C:P; SNP – soil N:P; SAN – soil available nitrogen; SAP – soil available phosphorus. BG, NAG, LAP, and AP indicate β-1,4-glucosidase, β-1,4-N-acetylglucosaminidase, leucine aminopeptidase, and acid phosphatase, respectively.
Conclusions
Our study showed STN, SAN, SOC, soil C:N:P ratios, and the four soil EEAs increased with increasing stand age in I. verum plantations, while the contents of STP and SAP showed no significant changes. The soil ECN showed no significant difference with stand age, while the soil ECP and ENP both significantly decreased with increasing stand age. SWC and soil nutrients were major factors affecting the soil EEAs and stoichiometry in I. verum plantations. The soil enzymatic C:N:P ratio was 1:1:1.4, indicating soil microorganisms were severely limited by P availability. Therefore, phosphate fertilizer should be applied to promote plant growth for stable and high fruit yield in I. verum plantations. Our results offer insights into the effect of forest plantation chronosequences on soil extracellular enzyme stoichiometry and nutrient limitation in tropical mountain areas.

