

Introduction
Weir gates are artificial structures that can be opened or closed to regulate water flows within a channel of flowing water. However, the barriers built across a river channel may pose a risk of deteriorating water quality as a repercussion of decreased water flow rates and increased hydraulic residence time that may lead to eutrophication and trigger algal blooms. Large rivers in particular often have substantial human-induced development in proximity to river margins, resulting in runoffs of both significant nonpoint (e.g., agricultural nutrients) and point (e.g., wastewater discharges) source pollution [1]. Much research has been devoted to understanding how man-made, regulated rivers had an effect on surface water quality associated with algal blooms and biomass accrual. An understudied feature that controls eutrophication and associated algal growths in managed waterbodies is variation in algal primary productivity in reflowing waterbodies following weir gate openings compared with standing waterbodies prior to weir gate openings. This information is critical for developing guidelines for weir gate operation aiming to mitigate eutrophication and unwanted algal blooms. Until recently, there have been few studies nationwide as well as worldwide (in particular, in northern temperate regions) to make a large-scale recovery assessment of reflowing rivers with a focus on algal primary productivity affected by weir gate operations.
In aquatic systems such as natural rivers, river weir impoundments (or dam reservoirs), and natural lakes, nitrogen (N) and phosphorus (P) play a pivotal role in algal growths and aquatic ecosystem function. In particular, knowledge concerning algal production per unit of total phosphorus (TP) (TP measurement is a universal way to measure P) is important for eutrophication control and water quality management, and the relationship of P with algal biomass has been widely considered to determine the waterbody trophic state [2, 3]. However, because different aquatic systems have different requirements of N and P for algal growth depending on algal community composition, it is crucial to understand the relative supply of N and P and whether they are growth-limiting nutrients for controlling primary productivity in natural and man-made aquatic environments as well [4]. In general, algal biomass (as estimated with chlorophyll a [Chl a]) has been found to depend more on P concentrations in temperate lakes and reservoirs or impoundments regionally or worldwide [5-7]. Because Korean freshwater systems are mostly P-limited (and N is sufficient), relating the amount of P to algal biomass is reasonable for determining algal nutrient limitation. Canfield and Bachmann (1981) noted that TP–Chl relationships did not vary with whether the lake is natural or artificial, but rather, abiotic and biotic factors including water temperature, hydraulic residence time, water flow rates, and aquatic biota other than TP may have a direct effect on algal growths [8]. In other words, geomorphological, hydrological, and biogeochemical variations that occur in and around aquatic systems are expected to differently mediate the responses of algal biomass to P concentration. Therefore, variation in the responses of algal growths to TP between the periods of closed and opened weir gate openings in a fluvial (riverine) ecosystem can point out not only the necessity of P reduction but also the control of other physiochemical factors that limit algal growths [9, 10].
Three large in-stream (river) weirs that were constructed across the main stem of the Geum River in South Korea between the headwaters and river mouth in 2012, primarily for the purposes of efficient water use and flood prevention, closed their weir gates until 2018 and then opened them after 2018 to aid eutrophication abatement and water quality improvement. Because few researchers had compared algal primary productivity affected by weir gate openings or closeness during a relatively long period of time, I tested how altered P supply carried by reflowing waters after weir gate openings would exert an impact on algal biomass accruals in the main stem of a large river in the northern temperate region. In South Korea, giant artificial barrier construction in the main stems of large rivers has been an enduring socioeconomic issue because of the potential for extensive algal blooms and biomass accrual and the resultant water quality deterioration. This may be a crucial issue in that the reduced flow rates derived from weir construction along with nutrient-enriched waters could be the main determinant for harmful algal blooms such as Microcystis or N2-fixing bacteria as well [11-14]. Although the Korean government in recent years has completely opened the weir gates and has been monitoring the ecological recovery of the reflowing status of large rivers following weir gate openings (there was some variation in opening time periods between weirs), the impacts on nutrient fluxes and primary productivity have not been fully investigated.
In this study, my goals were to compare empirical algal biomass–P concentration relationships among the waterbodies formed by weirs and dams (i.e., impoundments and reservoirs) in the same main stem of a large river to better understand a broad-scale variation in algal primary productivity that was caused by weirs’ altered hydrology. I will dedicate this regional case study to improving the knowledge of ecosystem processes and functions of a large reflowing river following full weir gate openings and thus offer integrated insights on eutrophication mitigation strategies for managed freshwater ecosystems. In this regard, I addressed the following 2 main questions: (1) Did continuous and full openings of weir gates over several years help improve the water quality of a large managed river by neutralizing the positive responses of algae to P concentration?
(2) How did algal biomass responses to P concentration shift from upstream to downstream along the main stem of the Geum River? Additionally, I tested if the TN:TP ratio can be considered an appropriate index for nutrient limitation in river impoundments and man-made lakes (dam reservoirs) in the northern temperate region.
Materials and Methods
Study Sites
The 3 middle-stream weirs, 1 estuary dam, and 1 upstream dam in the main stem of the Geum River in Chungnam province are located 300 km southwest of Seoul, the capital of South Korea, between 36°, 00–28’, 00–33” N, and 126–127°, 28–48’, 20–31” E (Fig. 1). The Geum River is 397 km long and typically 120 m-1,700 m wide. The river’s origin is the foothills of Sinmoo Mountain in Chonbook province, draining 11.582 km2. The river basin is subject to a temperate East Asian monsoon climate with heavy rains in the summer season (from July to September). A monsoon climate delivers about 50-60% of annual precipitation. The water quality of the Geum River was greatly affected by catchment land use practices where the dominant percentages of land use covers were forests, agriculture, and urban development in descending order [15, 16].
Fig. 1.
The 5 study waterbodies created by artificial structures (dams and weirs) in the main stem of the Geum River Basin (◼). Note: Sejong weir (the first middle-stream weir); Gongju weir (the second middle-stream weir); Baekjae weir (the bottommost weir).
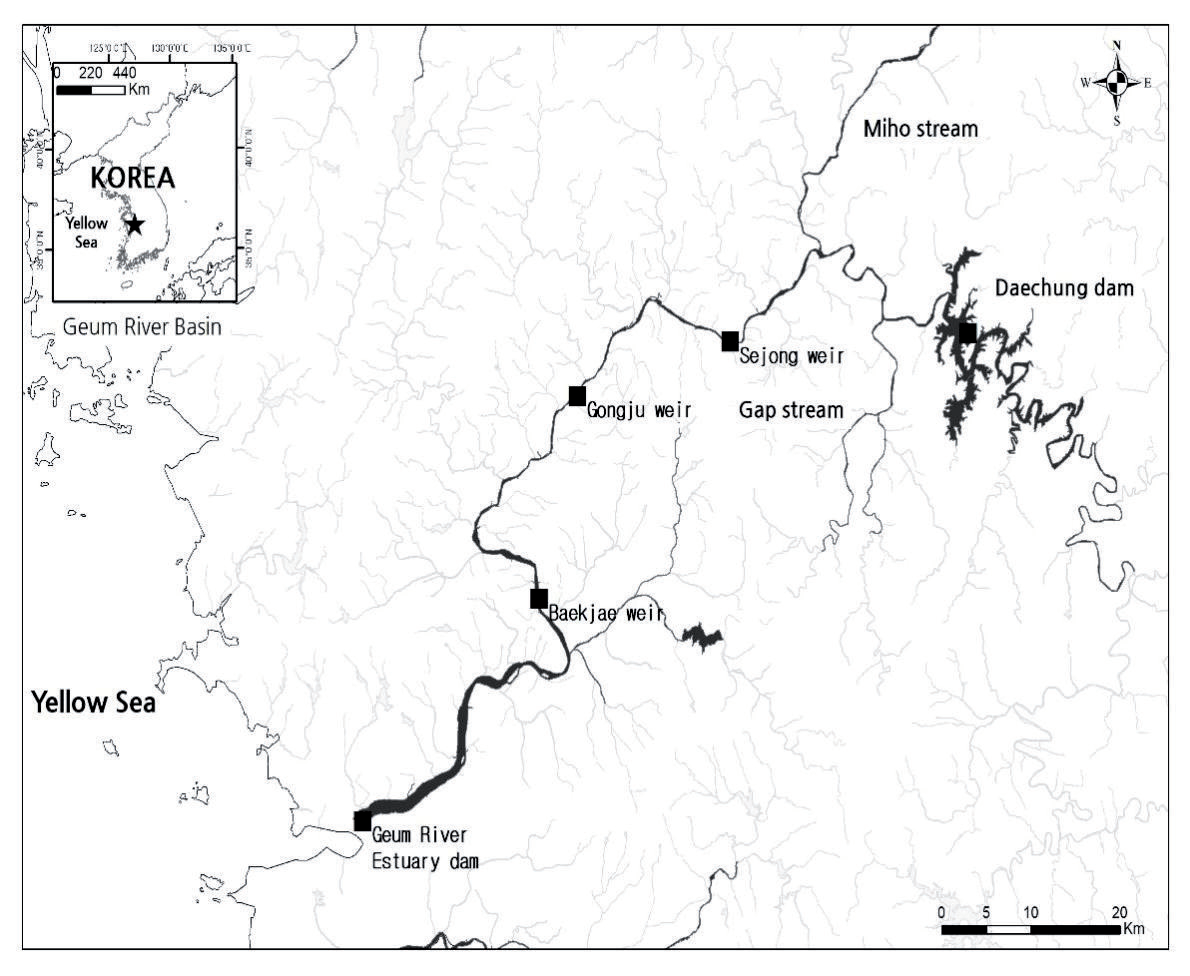
The 3 middle-stream (in-stream) weirs were constructed between 2009 and 2012, primarily for agricultural and domestic water use as well as flood prevention, whereas the upstream dam just above the uppermost weir was constructed in 1980 for multipurpose uses such as agricultural water use, potable water, flood prevention, and electricity generation. The waterbody created by the upstream dam (“Daechung Reservoir”) discharged waters from the dam’s gates twice every day, whereas the waters were discharged several times during the rainy summer season. From 30 tons (regular season) up to 60 tons of water per second (rainy season) were discharged from the dam’s gates at one time [17]. The estuary dam at the mouth of the Geum River was built in 1994 to control upstream flooding, especially in the rainy summer season, and to secure agricultural and industrial water uses [18]. The dam’s gates are usually opened once a day during summer and once every 2 or 3 days in winter. The gates are opened a few hours every day during ebb tide to prevent severe saltwater intrusion. Dam waters are discharged through sluice gates (gate bottoms are 5 m below sea level) during ebbs if the water level is higher than the estuarine side by more than 0.2 m or when flooding events occur. The estuary dam discharges about 6.4x10⁹ tons of river waters into the Yellow Sea every year [19].
More than 30 tributaries including the two largest ones in size, “Gap Stream” and “Miho Stream”, feed into the mainstem of the Geum River. The catchment land use that predominates in the drainage basin of the upstream dam was forested, while the catchments of the estuary dam were primarily occupied by agricultural fields like rice paddies and other crop fields. In particular, the drainage basin of the upstream dam was protected lawfully for a drinking water source with strict development restrictions. The drainage basin of middle-stream weirs was dominated by forests, agricultural fields, and urban areas in descending order. The two largest tributaries, “Gap Stream” and “Miho Stream”, located downstream of the upstream dam that feeds into the upstream of Sejong Weir, were considered a major contributor to both nonpoint and point source pollution from watersheds in the study waterbodies [17].
According to the data publicly available, the mean nutrient (N, P) concentrations in the mainstem of the Geum River in the 2005-2007 years (prior to weir construction) were higher than those of both closed and opened-gate periods of weir gates (2015 to 2017; 2019 to 2022). Meanwhile, SS concentration in the 2005-2007 years was higher than the closed periods, but lower than the opened periods of weir gates [20].
Data Collection and Analyses
I made the comparison of physiochemical and biological features of the study aquatic systems (waterbodies) between 2 separate time periods determined by whether weir gates were closed or opened (January 2015 to December 2017 vs January 2019 to December 2022). I obtained most data on hydraulic and morphometric characteristics of weir and dam waterbodies from the public database of the Water Resources Management Information System (www.wamis.or.kr) [15] and Korea Rural Community Corporation, where government scientists have regularly collected scientific data. In this study, I defined the water storage volume for a waterbody (formed by a weir or dam) as the amount of water (1) between the uppermost dam (not included in this study) and the upstream dam, (2) between the uppermost weir and its upstream dam, (3) between 3 middle-stream weirs, or (4) between the bottommost weir and its downstream estuary dam (at the river mouth), all in the same main stem of the Geum River. A hydraulic residence time for a waterbody (dam reservoir or weir impoundment) was its water storage volume (m3) divided by volumetric flow rate (m3/s). I calculated the mean water depth of the waterbody by dividing the water storage volume (m3) by its surface area (m2). I obtained the mean water velocity by dividing the volumetric flow rate (m3/s) by the river’s area (m2) in a channel’s cross-section [21]. Volumetric flow rate (m/s) was measured upstream of each individual waterbody. Because of heavy agricultural land use cover in the Geum River Basin, nutrient loading (N and P) oftentimes fuels algal blooms. Mean water depths and hydraulic residence time of the study waterbodies were reduced from 67% to 80% and 66% to 90%, respectively, after weir gate openings occurred [22] (Tables 1 and 2).
Of the large datasets publicly available on nutrients and sediment in water columns, I compiled the 2 most crucial nutrients (i.e., total nitrogen (TN) and total phosphorus (TP)) and sediment (total suspended solids (SS)) for aquatic photosynthesis and primary productivity from the National Institute of Environmental Research’s web portal (https://water.nier.go.kr) under the Korean Ministry of Environment (KMOE). For the data collection, the relevant government scientists take the daily or weekly water samples for a waterbody, and the physiochemical and biological parameters selected for this study were TN, TP, SS, and Chl a (Chlorophyll a).
The government scientists took water samples during daylight from a water column about 500 m upstream from a weir or dam in ice-free seasons and analyzed the waters according to the KMOE’s (Korean Ministry of Environment) standard methods for the examination of water pollution [23]. A water chemistry value of a waterbody indicates the mean by the average of the daily or weekly samples collected and by averaging 1-6 sampling sites within a waterbody horizontally (weir impoundment), or by averaging 2 or 3 sampling sites with a waterbody (weir impoundment or dam reservoir when thermally stratified). Weir impoundment’s water samples were obtained usually at one third of the water depth, if the depth was less than 2 m, and a combined (mixed) sample of water was taken at one third and two thirds of the depth if the depth was more than 2 m. On a river cross section (weir impoundment), three sub-locations were sampled: one located in the maximum water depth, the second situated between the maximum and one side of a river bank, and the third between the maximum and the other side of a river bank. The upstream dam reservoir’s water samplings were carried out from the 3 vertical locations of a waterbody (epilimnion, metalimnion, and hypolimnion if thermally stratified; if not thermally stratified, the first sampling location occurred between the surface and the half depth of the whole dam reservoir, the second sampling location was at the half depth of the whole waterbody, and the third sampling location was placed between the half depth of the reservoir and the bottom).
Table 1.
The hydrologic and morphometric features of the 5 study waterbodies in the Geum River Basin, South Korea, during the period of closed weir gates (2015-2017).
Table 2.
The hydrologic and morphometric features of the 5 study waterbodies in the Geum River Basin, South Korea, during the period of opened weir gates (2019-2022).
Although there is some weakness for use [24] that is attributed to variation in algal pigment contents affected by environmental factors such as light penetration, temperature, and nutrient limitation, Chl a is still commonly used to measure algal biomass in aquatic ecosystems as a response variable because there is a close relationship between algal biomass and Chl a [25, 26]. According to the trophic states defined by Chl a concentration [27], the 5 study waterbodies are mesotrophic (7<Chl a<30 µg/l) or eutrophic (Chl a>30 µg/l).
I used a dataset of up to 6 years that comprised a closed period (January 2015 to December 2017) and an opened period of weir gates (January 2019 to December 2022) to assess how changes in the hydrologic regime induced by weir operation could have an impact on the response of algae to P, a primary limiting nutrient for algal growths, in the study aquatic ecosystems. For the study aim to be achieved, I made a comparison, especially for TN:TP and Chl:TP ratios of the 5 waterbodies along the Geum River’s main stem. A TN:TP ratio is often useful for determining the potential nutrient limitation of sestonic algae. For example, Maberly et al. [28] argued that P-deficient growth continued to occur when the TN:TP ratio was more than 20 (by molar ratio), whereas algal growth was N-limited when the TN:TP ratio was less than 10. A Chl:TP ratio (algal production yield per unit of TP) can be used to infer not only the likely response of algae to the primary limiting nutrient, P concentrations, but also environmental factors that control Chl a other than nutrient availability. For the comparison on durations of closed and opened weir gate openings as well as individual waterbodies and waterbody type comparisons, I estimated the means of daily or biweekly measurement of TN, TP, and Chl a concentrations, and also the Chl:TP and TN:TP ratios with the daily or weekly mean values of each individual waterbody of weirs and dams with the daily or biweekly averaged TN, TP, or Chl a values.
I tested all data for normal distribution and log transformed them if necessary. I adopted the nonparametric Kruskal–Wallis test if the log transformed data still did not fill the normal distribution requirement for comparisons between waterbody types [dam (reservoir) vs weir (impoundment)], weir gate operation (closed vs opened), or 5 individual waterbodies, especially focused on the Chl:TP ratio. I tested the homogeneity of variance with Bartlett’s test, and if the homogeneity of variance was not met, I used Welch’s t-test and pairwise Wilcoxon test as post hoc tests. I compared the relationships of Chl a with P concentrations (i.e., slopes) between waterbody types and weir waterbodies with analysis of covariance (ANCOVA) to determine any statistically significant difference in the responses of algae to P that might be affected by weir gate operation. I determined the level of statistical significance at p<0.05. I performed all statistical tests using JMP 17 software.
Results
Nutrients (N, P) and Total Suspended Solids (SS) Concentrations
Across the 5 study waterbodies, the dataset covered a range of TN (0.52~7.76 mg L–1), TP (0.001~0.514 mg L–1), and SS (0.2~41.0 mg L–1) concentrations during the closed period, as well as TN (0.78~6.53 mg L–1), TP (0.004~0.360 mg L–1), and SS (1.5~94.4 mg L–1) during the opened period of weir gates. Overall, mean TN, TP, and SS during the opened period were higher than those during the closed period of weir gates.
More specifically, the upstream dam reservoir during the opened period displayed significantly higher TN, TP, and SS concentrations than during the closed periods (t = -5.1503, p<0.0001; t = -6.1954, p<0.0001; t = -3.0061, p<0.0013, respectively). The second middle-stream weir impoundment (“Gongju”) during the opened period represented significantly higher TN and SS concentrations (t = -2.14225, p = 0.0330; t = -1.0078, p = 0.0234) than during the closed-gates period, and mean TP concentration during the opened period was greater than during the closed period. The bottommost weir impoundment (“Baekjae”) showed a significantly higher TP concentration during the opened period than during the closed period (t = - 4.5048, p<0.0001). Though there was no statistical difference, TN and SS concentrations during the opened period displayed higher mean concentrations than during the closed period of weir gates in the bottommost weir impoundment.
In the highest weir impoundment (“Sejong”), no TN, TP, or SS concentration was found significantly different between the two periods of weir gates (Table 3), although the mean TN, TP, and SS concentrations were higher during the opened period than the closed period of weir gates. In Geum River Estuary Dam Reservoir, SS concentrations represented significantly higher concentrations during the opened period compared to during the closed period (χ2 = 10.1659, p = 0.0014). Mean TP concentrations in the estuary dam reservoir during the opened period were clearly higher than those in the closed period (t = 1.5012, p = 0.068), although there was no statistically significant difference at p<0.05. TN concentrations showed no difference between the closed and opened periods of weir gates.
Algal Biomass (Chlorophyll a: Chl a)
On average, Chl a concentration was higher during the opened period in comparison to the closed period of weir gates. Spatially speaking, Chl a concentration during the closed period continued to rise from the upstream dam to the uppermost and second middle-stream weirs and then declined in the bottommost weir and further declined in the estuary dam. By contrast, Chl a concentration during the opened period has continued to increase as waters moved down from the upstream dam up to the bottommost weir. In other words, during the opened period of weir gates, Chl a concentration kept increasing from the upstream dam reservoir (“Daechung”) to all 3 middle-stream weirs and then decreased only in the estuary dam. That is, Chl a concentration increased to peak at the bottomland weir and then declined in the estuary dam.
Chl:TP Ratio
Like the spatial pattern of Chl a concentration displayed during the opened-gates period, the Chl:TP ratio also exhibited a distinctive spatial variation from upstream dam to estuarine dam along the river continuum, but the spatial patterns of the ratio were somewhat different than Chl a concentration. More specifically, the bottommost weir impoundment had the highest Chl:TP ratio during both closed and opened periods of weir gates (Fig. 2). Furthermore, like Chl a concentration, Chl:TP ratios of each individual waterbody during the opened period were lower than those during the closed period of weir gates. Based on the similar, but somewhat different spatial patterns displayed between Chl a concentration and Chl:TP ratio along the river continuum, it was likely that hydrologic conditions derived from weir operation played a pivotal role in differentiating the algal response to P between the two periods.
The similar spatial variation of Chl a concentration as the Chl:TP ratio from the headwaters to the river mouth, irrespective of whether weir gates were opened, also implies that P was certainly a limiting factor for algal abundance in a large river in a temperate Asian region. Yet, closed periods showed a higher mean Chl:TP ratio than that of opened periods of weir gates. The mean Chl:TP ratio (0.64) of the closed period remained higher than the mean Chl:TP ratio (0.54) of the closed period of weir gates (χ2 = −7.2969, p<0.0001) (Fig. 3). More specifically, all the Chl:TP ratios of each individual waterbody, which ranged from 0.02 to 0.96, during the opened period were lower than their counterparts during the closed period, which ranged from 0.01 to 6.60. This result suggests that algae in closed-gate waterbodies were more regulated by P than their counterpart in opened-gate waterbodies. Hydrologic conditions may have played a significant role in reducing Chl:TP ratios during the opened-gate period as compared to the closed-gate period.
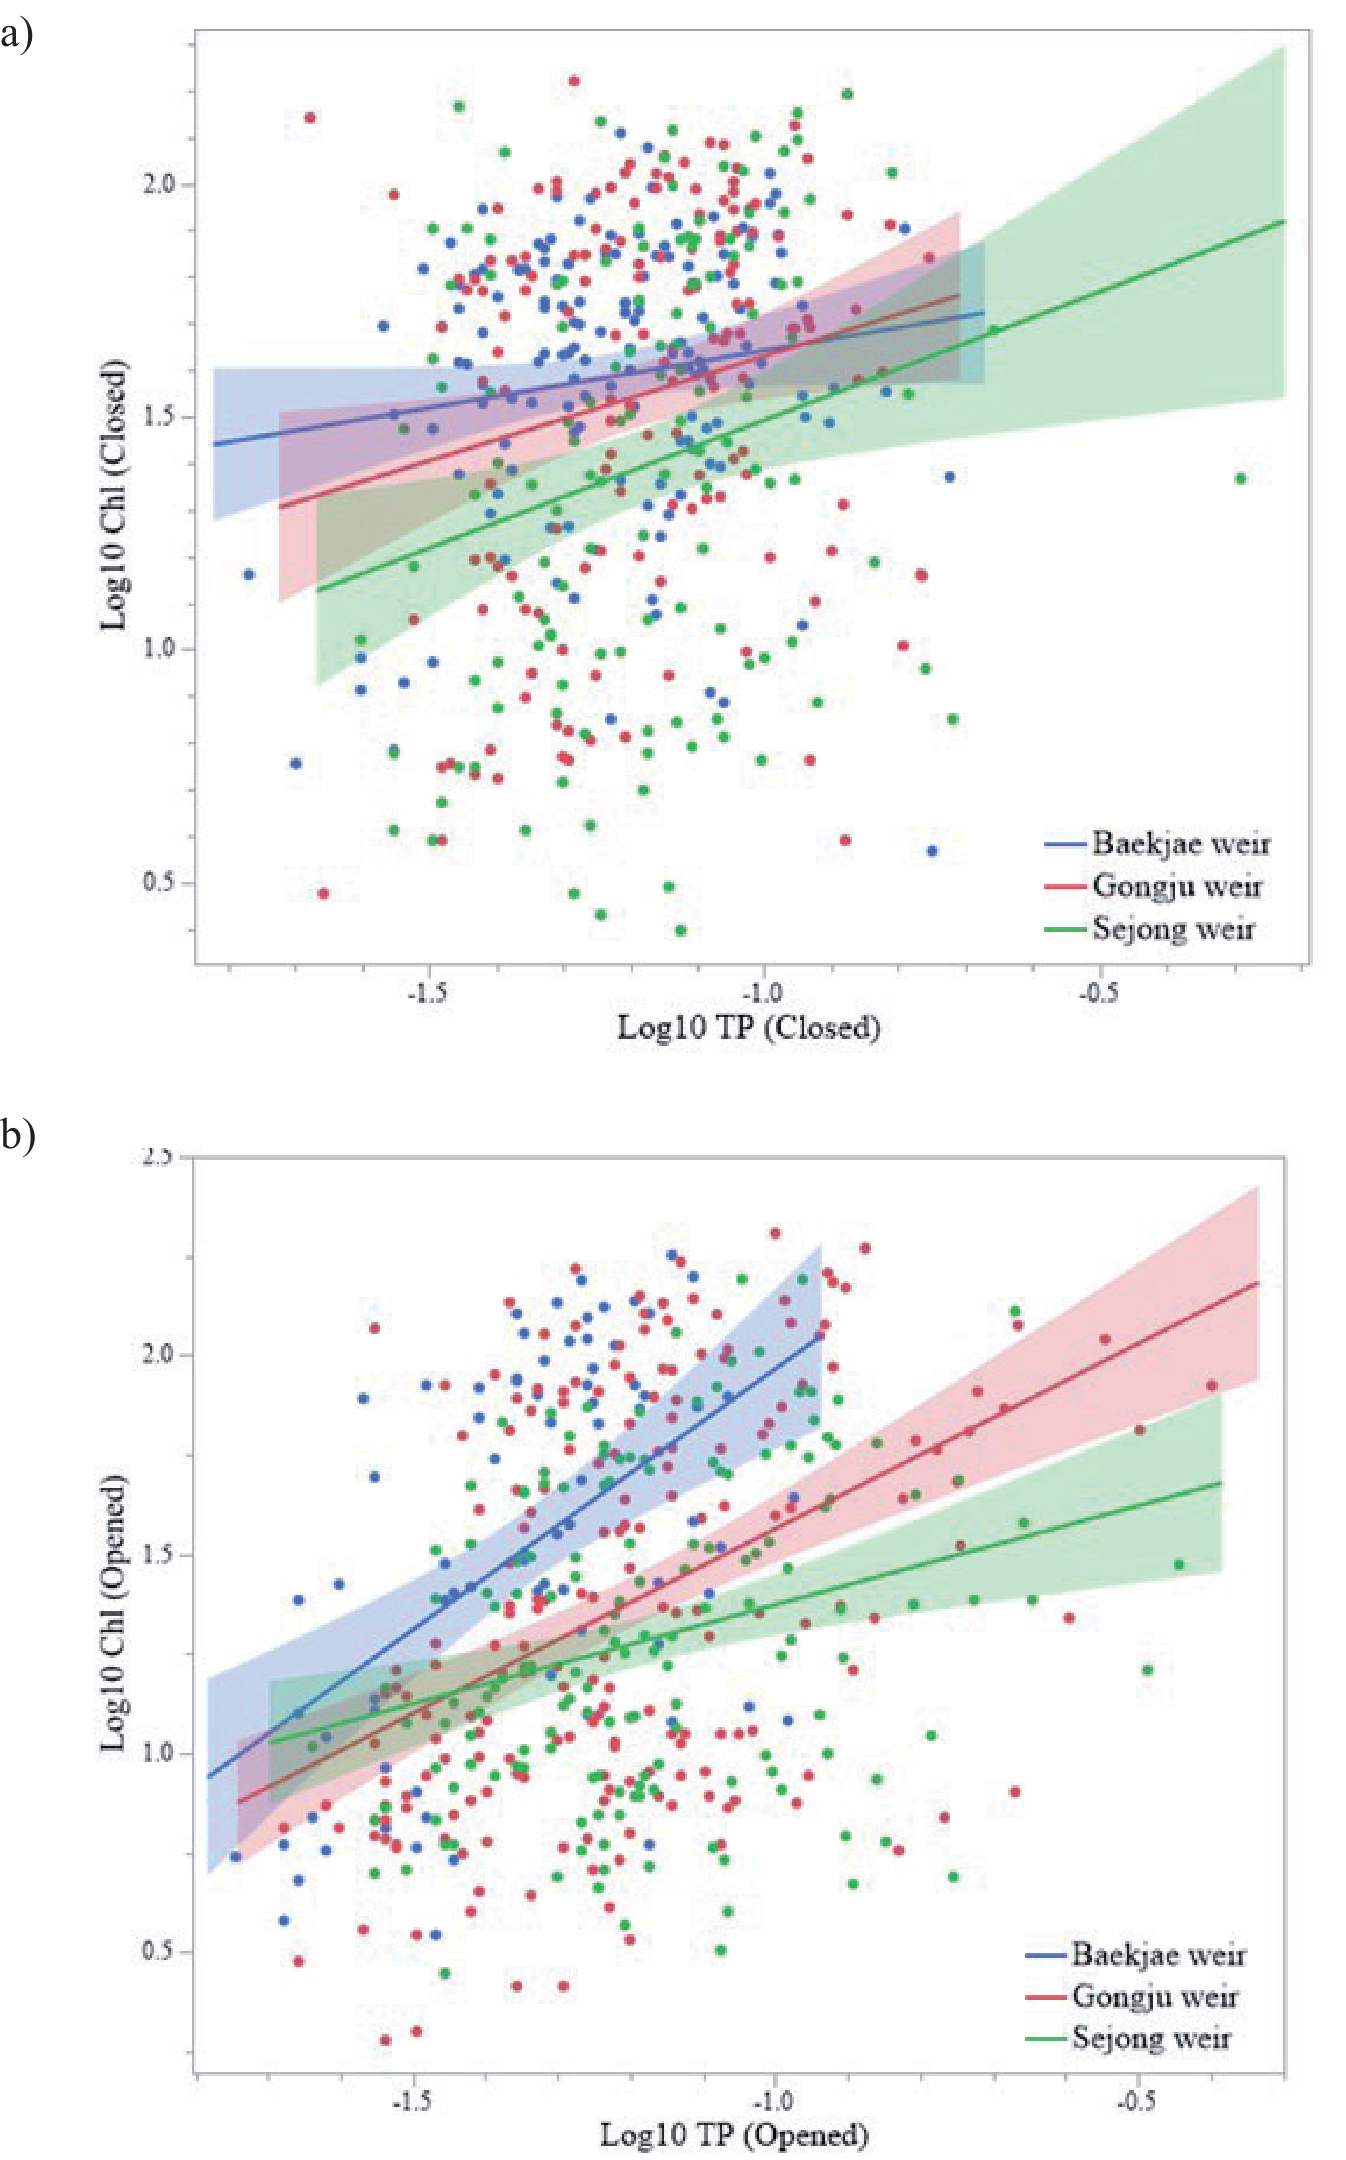
Regarding waterbody type variation, mean Chl:TP ratios of weir impoundments were significantly higher than those of dam reservoirs during both periods of closed (weir: 0.59 vs dam: 0.49) (χ2 = 27.0583, p<0.0001) and opened weir gates (weir: 0.55 vs dam: 0.47) (χ2 = 20.8520, p<0.0001) (Fig. 4). Furthermore, the among-weir (impoundments) variation during the opened-gate period was statistically significant (F = 4.3109, p = 0.0140) (Table 4; Fig. 5), in which the bottommost weir impoundment (“Baekjae”) differed from the first and the second middle-stream weir impoundments (“Sejong” and “Gongu”), respectively (t = 4.84, p<0.0001; t = 6.12, p<0.0001). Although the ratio’s difference between “Gongju” and “Sejong” weir impoundments was not considered “statistically significant” at the significance level of 0.05 (t = 2.12, p<0.0860), one could not conclude that the covariate (waterbody) was unlikely to affect the variation in the relationships between TP and Chl a concentration since the P value, whose threshold was arbitrary, was close to 0.05. Therefore, even if statistically insignificant, it is reasonable to say that the result was “scientifically significant” [29]. That is, the 2 middle-stream weir impoundments differed from each other in the response of Chl a to P concentrations following weir gate openings. However, during the closed period, the response of algae to P concentration (Chl:TP ratio) did not differ among the 3 middle-stream weir impoundments (F = 0.8037, p = 0.4484).
Fig. 2.
Log10 Chl:TP ratios compared between the 5 studied waterbodies during the durations of (a) closed weir gates (Geum River Estuary Dam: n = 77; Baekjae Weir: n = 145; Gongju Weir: n = 147; Sejong Weir: n =133; Daechung Dam: n = 565) and (b) opened weir gates (Geum River Estuary Dam: n = 45; Baekjae Weir: n = 77; Gongju Weir: n = 200; Sejong Weir: n = 161; Daechung Dam: n = 525). Box plots with means (middle horizontal lines) and 95% CI error bars. The bottom and top of the box are the first (25%) and third (75%) quartiles. Bars within boxes represent the median value, and error bars indicate one standard deviation.
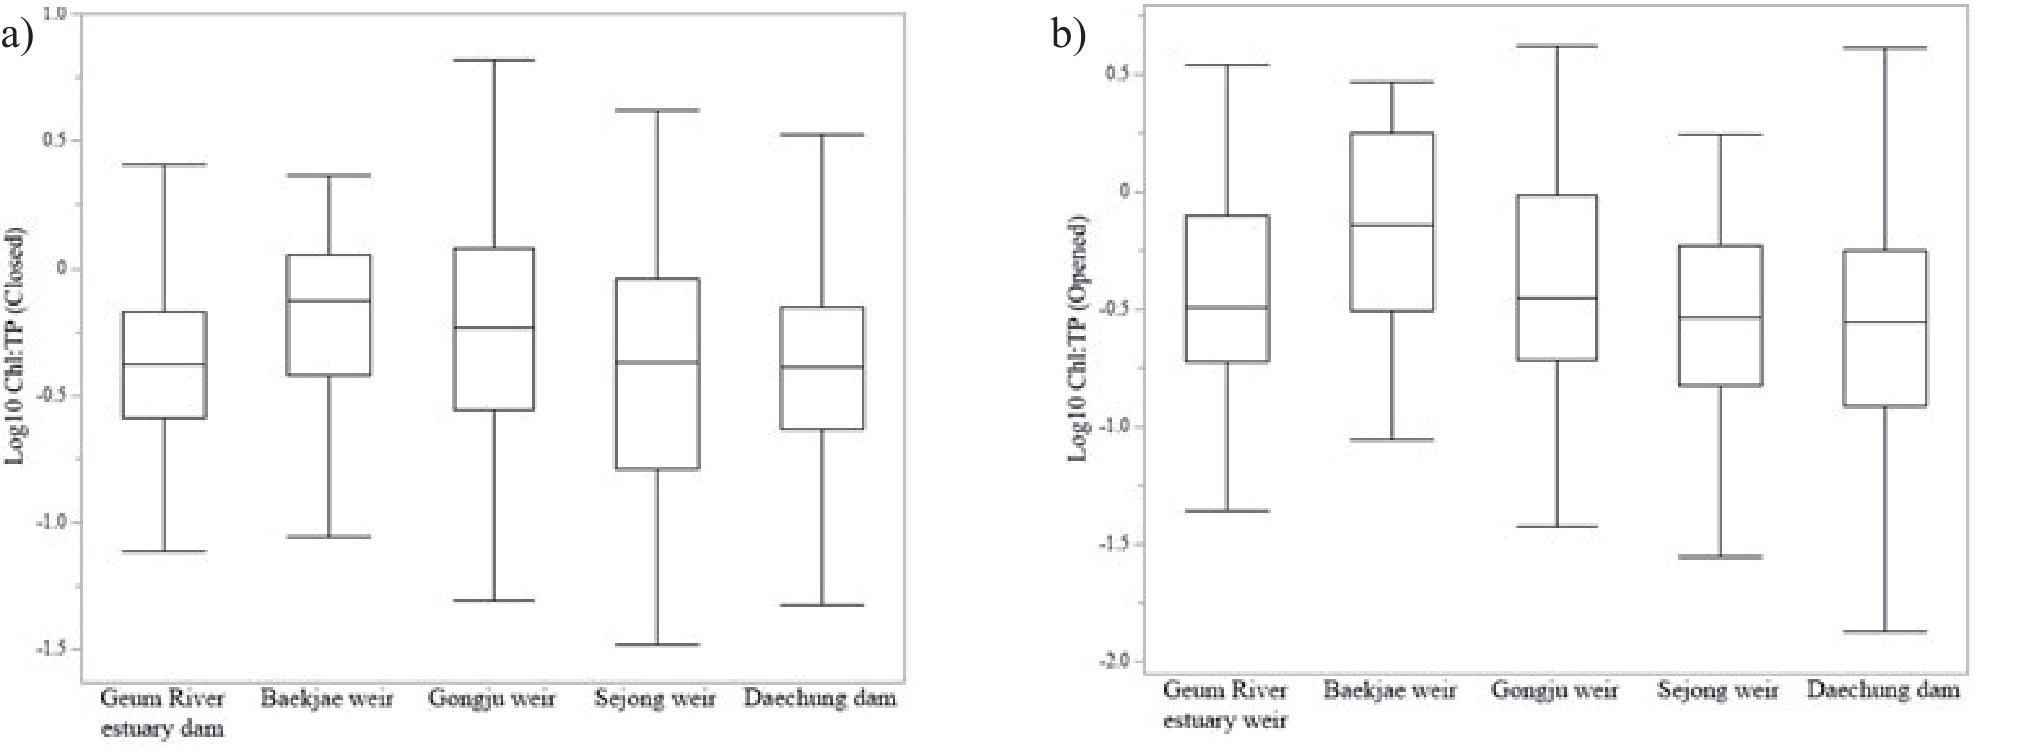
Fig 3.
Log10 Chl:TP ratios compared between the durations of closed weir gates (dam: n = 641; weir: n = 525) and opened weir gates (dam: n = 570; weir: n = 438). Box plots with means (middle horizontal lines) and 95% CI error bars. The bottom and top of the box are the first (25%) and third (75%) quartiles. Bars within boxes represent the median value, and error bars indicate one standard deviation.
TN:TP Ratio
The lower TN and TP concentrations were observed in the upstream dam reservoir (“Daechung”) with strict development inhibition in comparison to middle-stream weir impoundments as well as the estuary dam reservoir during both opened and closed-gate periods. The waterbody (reservoir) of the upstream dam, in particular, was 4-5 times lower in TP than the other study waterbodies, whereas TN of the upstream dam was 2-3 times lower than the other study waterbodies. As a consequence, a comparatively higher TN:TP ratio was detected in the upstream dam reservoir than in any other managed waterbodies, irrespective of weir gate operation (opened or closed). By contrast, the estuary dam reservoir showed the lowest TN:TP ratio. This was because as waters moved downstream, P concentration was elevated by an increased chance of watershed (catchment) runoffs, while N can be lost from sedimentation processes such as denitrification.
Fig 4.
Log10 Chl:TP ratios compared between the waterbody types during the durations of a) closed weir gates (Dam: n = 639; Weir: n = 425) and b) opened weir gates (Dam: n = 570; Weir: n = 438). Box plots with means (middle horizontal lines) and 95% CI error bars. The bottom and top of the box are the first (25%) and third (75%) quartiles. Bars within boxes represent the median value, and error bars indicate one standard deviation.
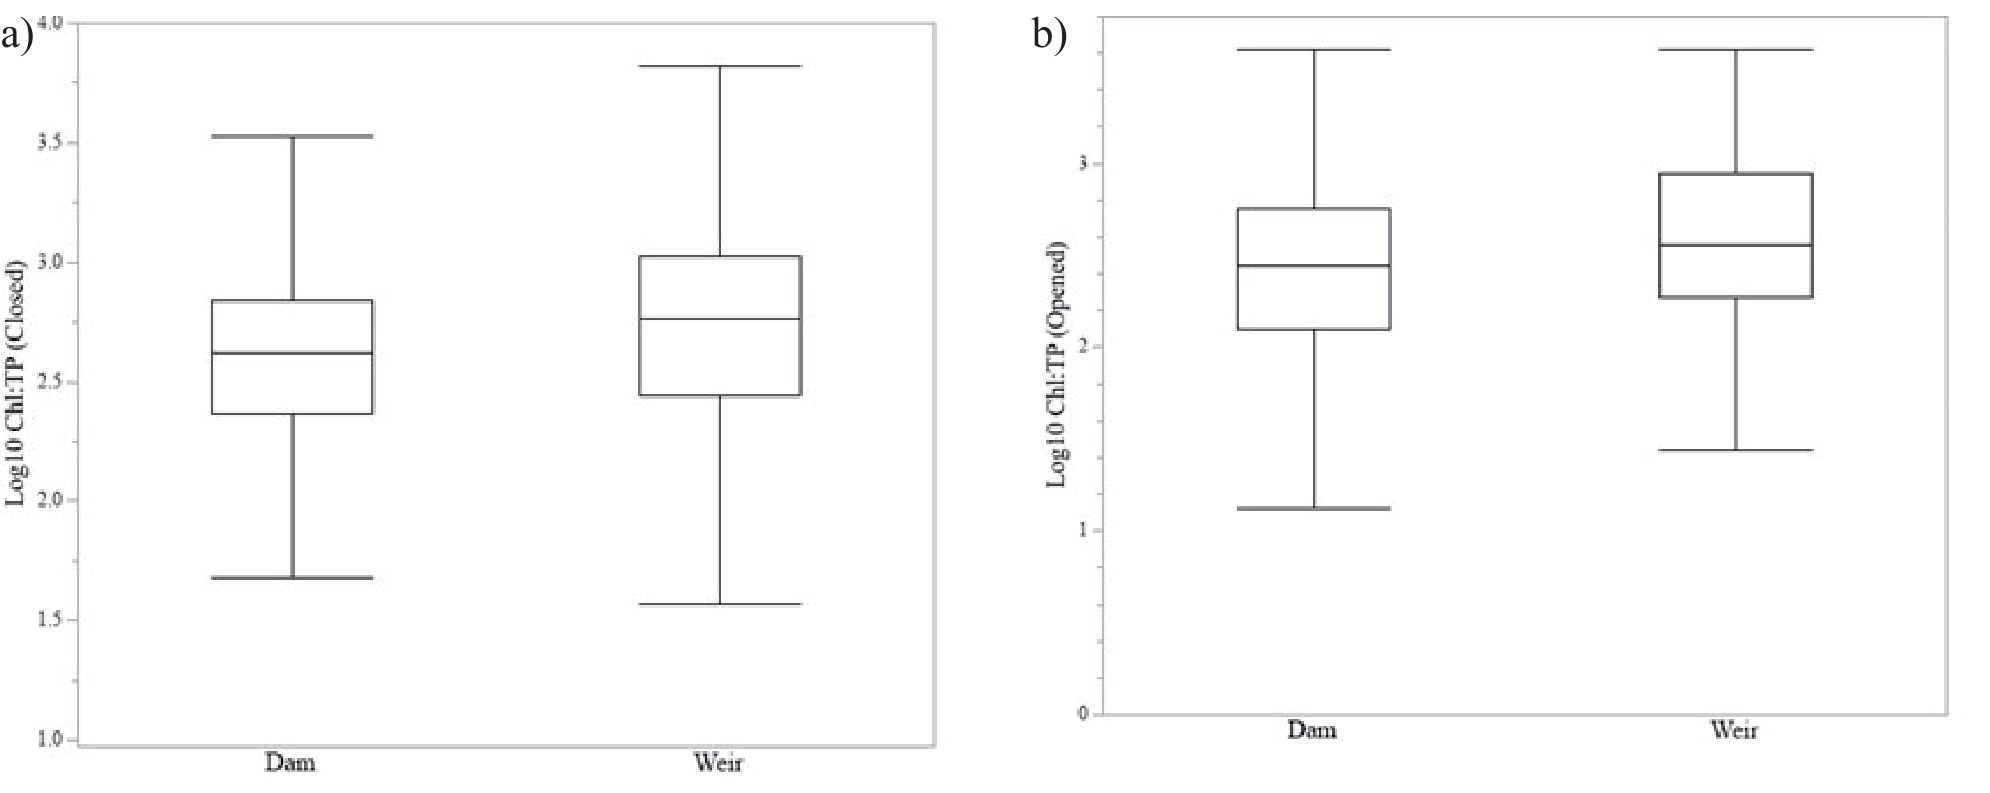
Fig. 5.
Comparison of the relationships (slopes) between log10 TP and log 10 Chl between weir impoundments during the closed a) and opened b) periods of weir gates from January 2015 to December 2017 (Closed) (top) and January 2019 to December 2022) (Opened) (bottom). Blue, red, and green ranges indicate 95 % confidence limits.
A higher TN:TP ratio in the upstream dam than 4 other waterbodies pointed out that P was retained in larger quantities in reservoir bottom sediments regardless of weir gate operation (closed or opened). Even though substantial amounts of water were discharged from the large dam during the rainy summer season, it is unlikely that significant amounts of P that had settled down in the bottom sediments in the upstream dam were recycled to the water column on account of the deep water levels maintained by the upstream dam operation [30], whereas the water column P in weir impoundments could have been easily moved from the bottom sediments due to wind and current forces that disrupted cohesion of bottom sediment in the waterbodies with shallow depths [31]. Thus, as a higher TN:TP ratio found in the upstream dam reservoir indicated, water column P in the deep dam reservoir seemed to be more likely to limit algal growths than weir impoundments regardless of weir gate operation.
Table 3.
Comparing the water chemistry parameters and Chl:TP and TN:TP ratios between the closed and the opened periods of weir gates.
[i] Note: Numbers in parentheses indicate the standard error of the mean (±) and range. TN (Total nitrogen), TP (Total phosphorus), SS (Total Suspended Solids), Chl (Chlorophyll a). The individual value of each parameter was based on a monthly mean of several water samples taken during a month. The Chl:TP ratio was calculated based on (µg L–1) in both Chl a and TP concentrations.
Discussion
Temporal and Spatial Variation in Nutrients and Algal Biomass
My goal in this study was to tie the altered hydrologic regime induced by weir gate operation to the algal nutrient limitation on a broad temporal and spatial scale in a northern temperate region. By using the publicly available datasets and appropriate statistical approach, I was able to elucidate the relationships of nutrient concentrations with algal biomass and its implications for surface water quality management following weir gate openings. On average, both TN and TP concentrations were higher during the opened period compared with the closed period of weir gates. Because the agricultural river basin is prone to soil erosion and surface runoffs, and P is mostly associated with soil particles, more nutrients were likely flushed out by soils and sediments following weir gate openings. Researchers have proved that increases in suspended solids (SS) concentrations were positively related to water column TP concentrations, suggesting that scouring and resuspension of soils and sediments brought P-adsorbed sediments (i.e., P attached to soils and sediments) into water columns during the opened period, especially in the rainy summer season [32]. In this study, SS concentrations in the 5 studied waterbodies have increased following weir gate openings (i.e., during the opened-gates period).
Table 4.
Comparison among weir waterbodies in the response of Chl a to P (ANCOVA).
The among-waterbody variation in Chl:TP ratio, especially among weir impoundments, suggests that water-column algal productivities in the study weir impoundments were negatively and differentially affected by turbid and scouring waters following weir gate openings. In addition, the response of Chl a to P concentrations has substantially increased as waters moved downstream. In other words, gate openings resulted in differential responses of algal biomass to P concentration among weir impoundments in the same main stem of the river, indicating that the strength of P in regulating Chl a concentration has been differentiated among weir impoundments and has increased as waters moved downstream. Considering unstable water column status following weir gate openings, which caused spatial complexity and hydrodynamic heterogeneity within the river’s main stem, reflowing waters were more likely to induce differential Chl–P relationships among weir impoundments. However, not only during the opened period but also the closed period of weir gates, the abrupt drop from the bottommost weir impoundment to the estuary dam reservoir in the Chl:TP ratio might have been because N limitation likely occurred as a result of denitrification that took place in the bottom sediments of the shallow and standing waterbody of the estuary dam, whereas P release from the bottom sediments likely has been enhanced in the presence of salinity and SO42- [30]. This repercussion also led to a lower TN:TP ratio, and P played a minor role relative to N in limiting algal productivity in the estuary dam (i.e., reservoir).
Why Did Weir Impoundments Have a Higher Chl:TP Ratio Than Dam Reservoirs Did? (Weirs vs Dams)
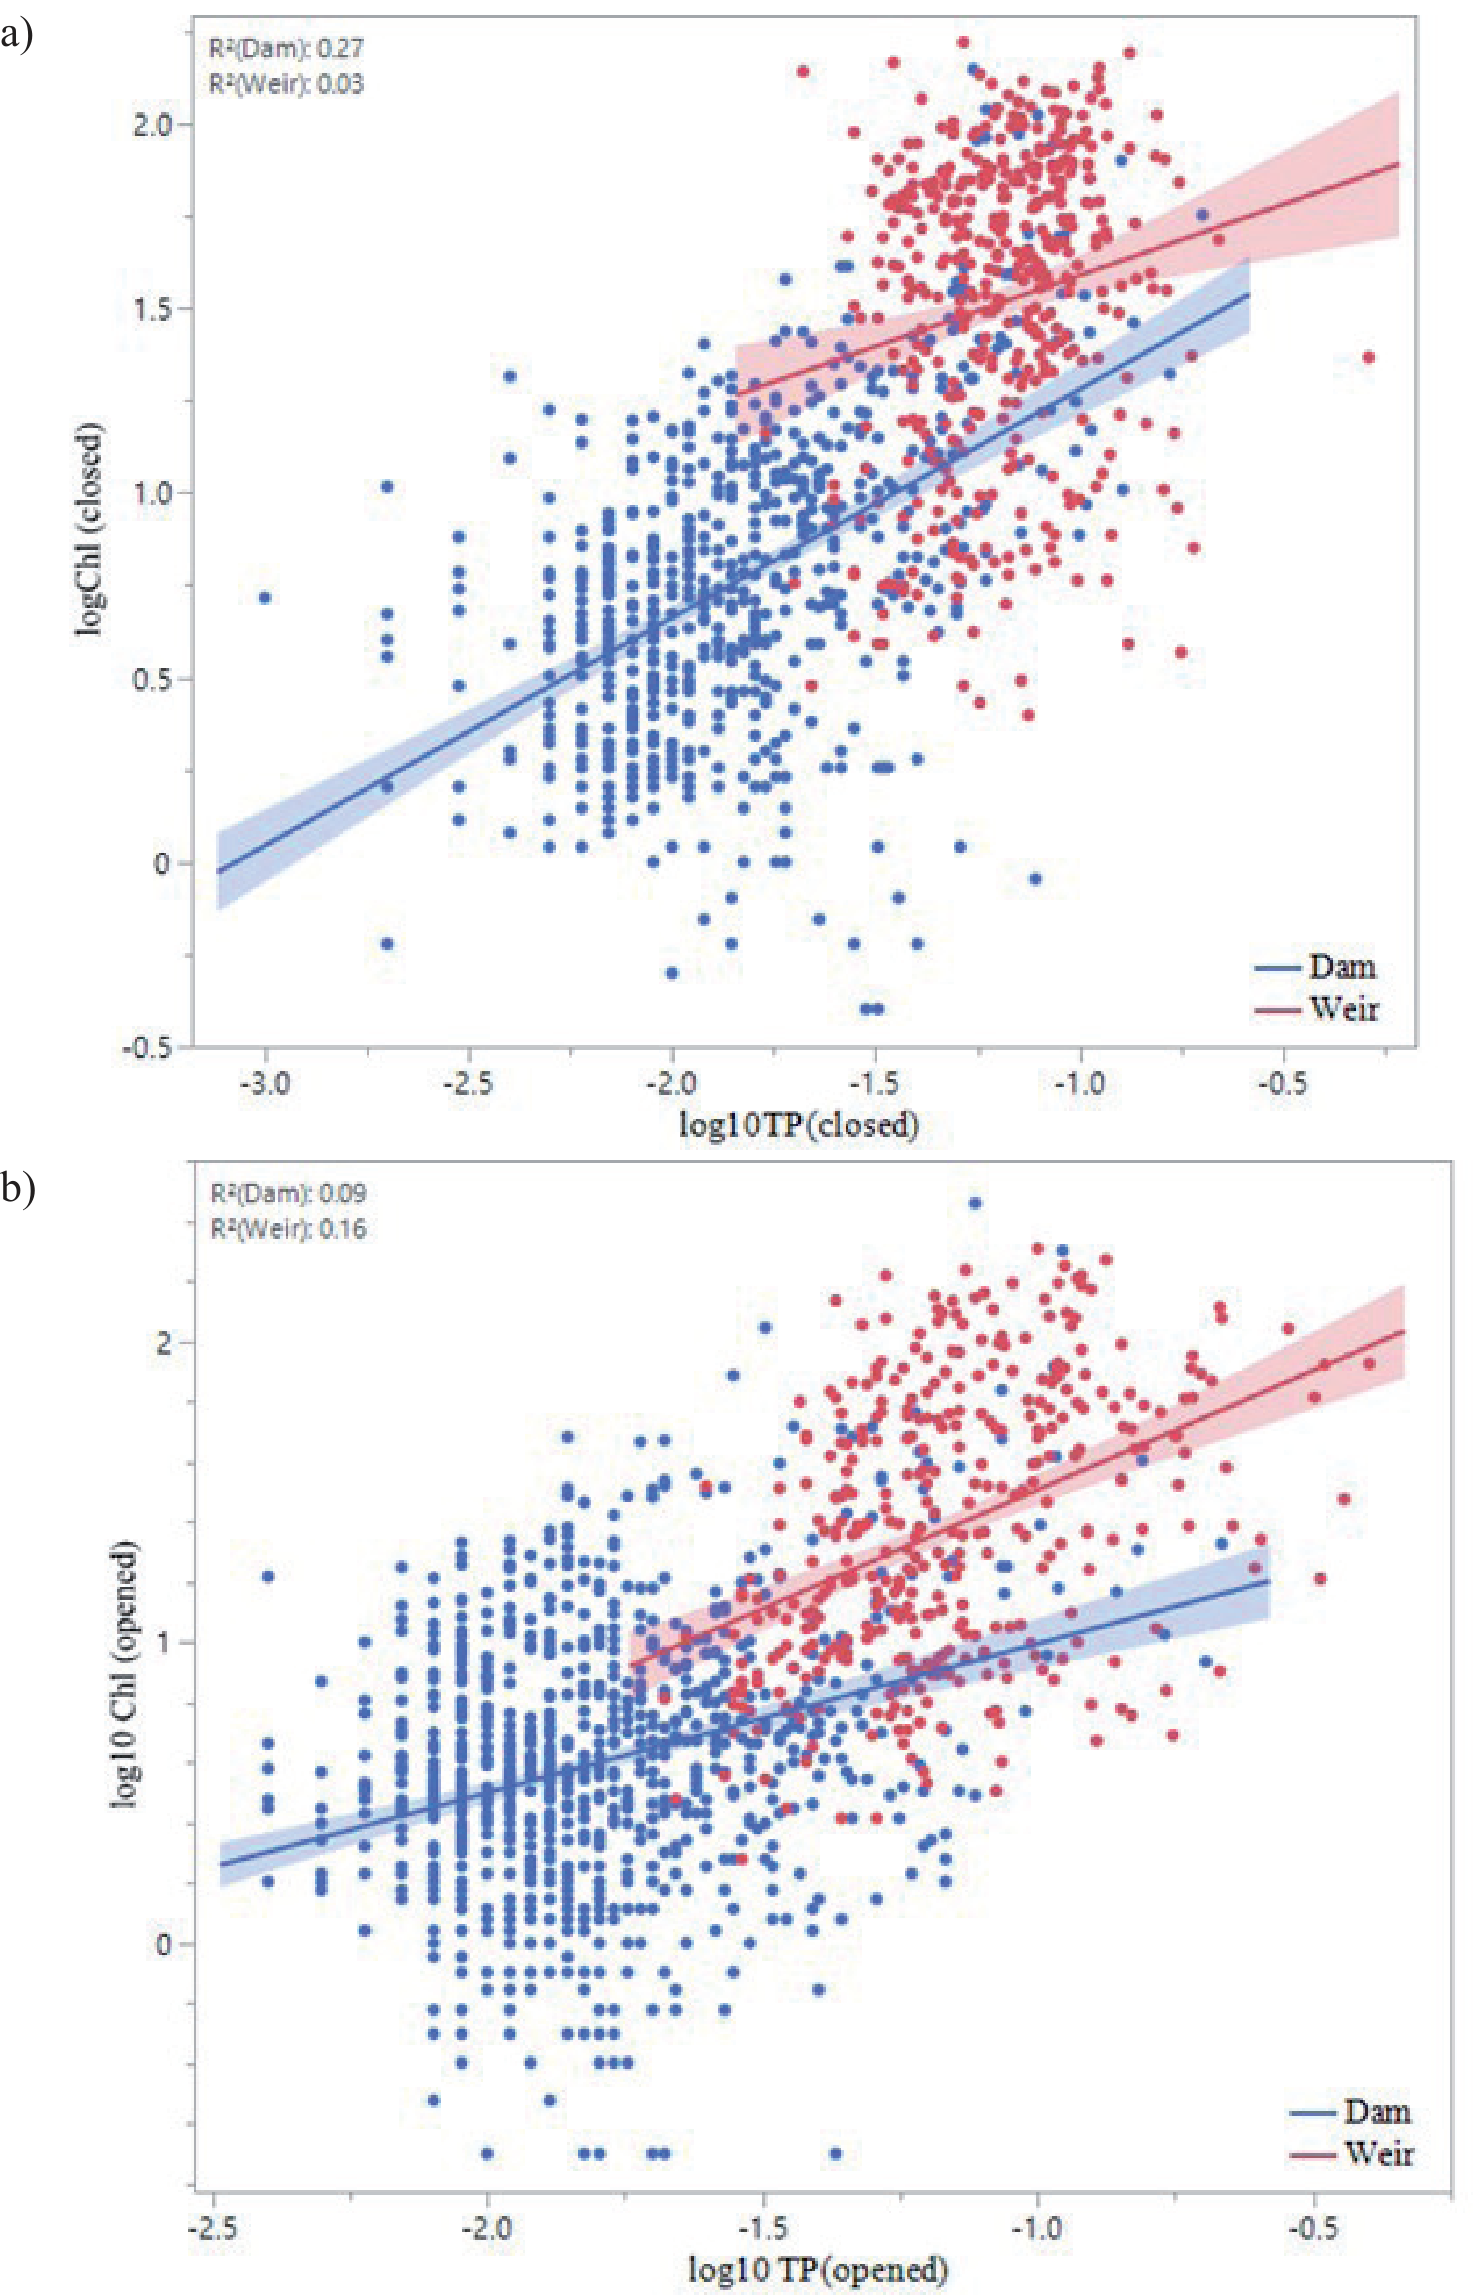
Researchers have used the ratio of Chl:TP to identify the environmental factors that limit algal growths other than P concentrations [31, 33] because the dependence of P to Chl a concentration (molar ratio) is used to identify aquatic trophic state and explain underlying ecological interactions between aquatic biota. The ratio between algal biomass (Chl a) and total phosphorus (TP) concentration, in particular, has been adopted to indicate the degree of eutrophication and algal blooms and is critical for eutrophication control and water quality management. To explain the effects of weir gate openings on algal primary productivity, I hypothesized that weir impoundments would have a lower mean Chl:TP ratio (i.e., lower TP to Chl transfer efficiency) than dam reservoirs, mainly because of hydrologic constraint derived from flushing waters and associated light limitation on algal biomass accruals that took place in weir impoundments during the opened-gate period of weir gates. In other words, increased water velocity and turbidity as well as reduced hydraulic residence time by scouring waters in weirs during the opened period may have a negative impact on algal growths and biomass accrual in the flowing waterbodies [34]. First, attenuated lights caused by non-algal water turbidity in flowing waters could limit algal growth to the point at which P supply exceeds the nutrient demand and preclude nutrient limitation that resulted in a lower ratio of algal biomass (Chl a) to P concentration. Light attenuation becomes greater with increasing nutrient availability as waters flow out downstream and receive more terrestrial nutrients from watersheds [35]. Second, benthic algae (periphyton) that grow on mud, rocks, and vegetation are a major part of algal communities in flowing waters [36]. However, because water samplings of weir impoundment took place in the water column only, the quantitative contribution of benthic algae to primary productivity can be overlooked. Thus, TP–Chl relationships were underestimated in the weir waterbodies (impoundments). Third, the amount of soluble reactive phosphate (SRP: labile form of phosphorus (P) taken up directly by algae) likely reduced in weir impoundments, which supplied more oxygen with high flow velocities and a low water table (depth) compared to dam reservoirs because SRP release from sediments to the water column is favorable in anoxic conditions, which should be more commonly found in lentic bottom sediments of dam reservoirs with low flow velocities and a high water table (depth) [37]. Increased discharge following weir gate openings was more likely to induce a smaller amount of SRP available to algae under increased oxygen levels in the flowing waters. As an experimental example, the amount of SRP has decreased at high discharge in subalpine streams in the United States [38]. Hence, it seemed reasonable that the relationships between Chl a and TP concentrations in dam reservoirs were found to be different than the relationships in weir impoundments during the closed-gate period (Fig. 6).
However, contrary to the predictions, mean Chl:TP ratios of weir impoundments were significantly higher than dam reservoirs during both periods of closed and opened weir gates. Turbidity-induced light limitation caused by flushing waters from opened weir gates might have been offset by shallow water depths, which might have helped enhance light intrusion and improve photosynthesis. Shallow water depths in the impoundments formed by weirs could allow algae to receive more light in the water column than the reservoirs created by weirs with a deep water level. Rather, light limitation had an adverse effect on the algal productivity of the upstream dam reservoir where water samplings were carried out vertically throughout the water column. Likewise, Spears et al. [31] found a lower likelihood of P limitation of algae with decreasing depth by their Chl:TP ratio analysis with 94 UK and Irish lakes. Shallow water depths of weir impoundments, especially during the opened-gates period, enabled planktonic algae to expose themselves to more light availability and a sufficient photoperiod, compared to the closed-gates period. In contrast, more flushing waters that flowed out from the upstream dam during the opened-gates period would not have been conducive to algal growth, presumably because of a hydrodynamic instability that was unfavorable to algal growths in dam reservoirs [39]. In this study, the mean water depth of dam reservoirs remained at more than 40 m for most of the study years, whereas that of weir impoundments was less than 10 m even during the closed period of weir gates. The shallow water depths of weir impoundments likely allowed for water penetration that was conducive to algal growths. Moreover, slow velocity in weir impoundments, regardless of whether weir gates were closed or opened, also offered optimum conditions for algae to proliferate.
Fig. 6.
Comparison of the relationships (slopes) between log 10 TP and log10 Chl between waterbody types (dam vs weir) during the closed a) and opened b) periods of weir gates from January 2015 to December 2017 (closed) (top) and January 2019 to December 2022 (opened) (bottom). Blue and red ranges indicate 95 confidence limits.
Soballe and Kimmel [40] noted that algal abundance (production) per unit P of natural lakes or river impoundments was higher than rivers, owing primarily to differences in water (hydraulic) residence time. This was because horizontal water movements control the time available for algae to interact with nutrients. (Rapidly) flushed ecosystems are less likely to permit algae to grow within a sufficient time frame. However, these researchers also found that the negative effects of rapidly flushing waters on algal productivity were significant in aquatic systems with a hydraulic residence time of less than 60~100 days. In other words, longer hydraulic residence time can offset the negative effect of the flushing waters on algal productivity. In this study, I detected a very short hydraulic residence time in weir impoundments (<3 days) even during the closed-gates period, and other major hydrologic factors (i.e., water depths and flow rates) did not play a pivotal role in reducing algal productivity either. In fact, water depths were low, and flow rates were still slow even after opening the weir gates. Although the positive responses of algal biomass to P concentration during the opened-gates period certainly became attenuated, Chl:TP ratios did not substantially decline relative to the closed–gates period for 4 reasons. First, it is most likely that hydraulic residence time or water flow rates were not sufficiently different to significantly induce the differential responses of algae to P between the periods of closed and opened weir gates. Second, a higher-than-expected Chl:TP ratio estimated in weir impoundments was also relevant to Vannote et al.’s River Continuum Concept [41]. In the popular scientific concept, because a river is wider and its order increases, subsequently increased light and nutrient levels and longer hydraulic residence time may have caused increases in algal yield (production) per unit TP. Third, the bottommost weir (“Baekjae”) just above the Geum River Estuary Dam had a higher Chl:TP ratio during the opened flowing period than the closed standing period of weir gates. This was because of a large influx of P through the weir gates from upstream, but P eventually settled down in the estuary dam because the dam physically blocked the water flows from the upstream weirs so that P in the dam was unlikely to play the same role as P in the bottommost weir in fueling algal growths. Fourth, intensive sediment resuspension induced by wind, current, or bottom shear pressure produced by flushing waters in the shallow waterbodies of weirs may have contributed to P release from bottom sediments and also brought sedimented algae back to the water column [42].
Why Was an Opened Period Lower than a Closed Period in the Chl:TP Ratio (Opened vs Closed)?
Opening weir gates appeared to provide an unfavorable condition for algal biomass accruals. It was reasonable to see a lower Chl:TP ratio during the opened period because the intervention of hydrologic forces on algal biomass accrual was likely greater in opened-gate waterbodies than closed-gate waterbodies. Reflowing and flushing waters through weir gates may have negatively affected the ability of the biota to uptake and utilize P in the unstable hydrodynamic status. However, despite the lower ratio of Chl a to TP following weir gate openings, the Chl:TP ratio (>0.5), on average, still pointed out that P was a major driver of algal biomass and abundance in South Korea’s regulated large river ecosystem when compared to the freshwater systems in other temperate regions of the world [40]. That is, it is likely that hydrologic alteration following weir gate openings did not significantly mediate the response of algae to TP.
Spears et al. [31] reported that the water column Chl:TP ratio across 94 UK and Irish lakes ranged from 0.02 to 0.96, displaying considerable variation in the strength of P limitation for phytoplankton biomass. They also noticed that there was significant lake-type variation in the Chl:TP ratio, in which lake types were classified based on water depth and alkalinity. The authors showed that the Chl:TP ratio increased with decreasing depth and moderate alkalinity levels. My study covered a wider range of Chl:TP ratios than their ratios as described earlier, which may suggest a greater variability in the strength of P as a main driver of algal biomass. For waterbody-type comparison, dam reservoirs had a significantly lower Chl:TP ratio than weir impoundments, which was in agreement with Spears et al.’s findings with regard to the relationships between Chl:TP ratio and water depth. Because of a much deeper mean water depth of dam reservoirs compared to weir impoundments, the ratio of Chl a to TP in dam reservoirs exhibited a much lower Chl:TP ratio than those in weir impoundments.
In particular, the bottommost weir impoundment (“Baekjae”) displayed a considerably high Chl:TP ratio (>1) even during the opened-gates period, implying a strong P limitation of algal biomass accrual in the flowing waters with hydrologic or geomorphological conditions not being a determinant factor of influencing algal abundance. Indeed, the Chl:TP ratio (1.07) during the opened period was unexpectedly higher than the counterpart (0.82) during the closed period of weir gates. This was perhaps because slow water velocity and reduced hydraulic residence time were not advantageous in reducing the positive responses of Chl a to P concentrations. Rather, bottom resuspension likely played a crucial role in recycling substantial P into the water column, which provides a favorable condition for algal growths in the weir impoundment. The Chl:TP ratio of the bottommost weir impoundment corresponded well with the results of another published study on the relationships between trophic status, Chl a, and TP in a temperate region. According to Jones et al. [43], the maximum chlorophyll a (Chl a max):TP ratio rapidly increased between oligotrophic and mesotrophic status, and it was highest throughout the eutrophic range and subsequently declined under hypereutrophic status in reservoirs in Missouri, United States (>125 µg L–1). In this study, mean 49 µg L–1 (TP) during opened periods of weir gates indicated that the average trophic status of weir impoundment belonged to “eutrophic”, where the highest Chl:TP ratio was found. However, considering the mean Chl:TP ratio (>0.57) in this study, P seemed to be a stronger driver for limiting algal biomass than other temperate lentic systems, where the mean Chl:TP ratio in Missouri reservoirs was 0.44 and UK lakes showed mean values of less than 0.4 [31].
Among-weirs variation in Chl:TP ratio may suggest that variation in flow paths following weir gate openings along a longitudinal gradient of the river likely enabled the reflowing waters to represent differential responses to P enrichment in the Geum River main stem, whereas, during the closed-gate period, the effects of P concentration on algal biomass seemed to be similar among weir impoundments. As waters move downstream after weir gate openings, various habitats such as sandbars and oxbows are created by lower water levels, owing to deposits of sands, silts, and sediments that were delivered by inflowing waters through opened weir gates. Sandbars and oxbows formed by reflowing waters have increased geomorphological diversity in rivers and could have brought about changes in the response of algal communities to nutrients under a renewed hydrodynamic regime. In addition, the flushing waters under low water levels likely allowed the uneven lifting of bottom sediments from the river bed, and this repercussion also induced topographical and biogeochemical heterogeneity among the weirs. In the meantime, currents and winds permitted sediments and waters to interact with each other, internal nutrient cycling occurred in weirs with shallow depths, and diverse water–sediment relationships in various topographical features on the river bottom also could have allowed for variation in P concentration among weir waterbodies because the nutrient is recycled back to the water column through bottom resuspension [44]. Sandbars, in particular, were reported to enhance not only topographical and biogeochemical heterogeneity [45, 46], but also the abundance of endangered species such as the “Korean tiger lizard” (Eremias argus) upstream of the bottommost weir impoundment (“Baekjae”) following weir gate openings [47].
In the meantime, closed weirs may have played a role in attenuating the impacts of flow paths from upstream by making weir waterbodies topographically and ecologically homogeneous. This is because high water levels, which are anticipated to be less influenced by winds and currents that can cause bottom nutrient resuspension, may have eliminated a variety of habitats downstream by submerging them. Altered landscapes by weir construction that erased virtually all of the geomorphologically diverse habitats may also have enabled biogeochemically homogeneous TP–Chl relationships among the weir impoundments.
In addition, distinctive dissimilarities in terms of geohydrology and limnology between the waterbodies created by dams and weirs were accountable for the between-type difference in the algal biomass–P relationships. However, as noted in Fig. 7, the response patterns of Chl to TP concentrations in the Geum River’s main stem during the opened-gate period were sigmoidal, not linear. In other words, TP concentration increased from 0 to 1 mg L–1 linearly with a near-flat response between 1.5 mg L–1 and 2.5 mg L–1 and then declined as P concentration further increased. This observation was consistent with other findings [31, 48-51] in northern temperate lentic ecosystems of the world where TP–Chl relationships in published studies were sigmoidal or not linear, suggesting that the lentic ecosystems were not necessarily no longer limited by certain TP concentrations. There, other environmental factors such as zooplankton grazing pressure have perhaps influenced Chl concentration. Or a second nutrient, N, may play a more vital role in algal biomass accruals (i.e., N-limited condition under P replete condition). Researchers reported that filamentous cyanobacteria were dominantly in abundance at intermediate TP concentrations [32, 50, 52].
Does the TN:TP Ratio Serve Well as an Indicator for Controlling Algal Growths in a Human-Regulated River?
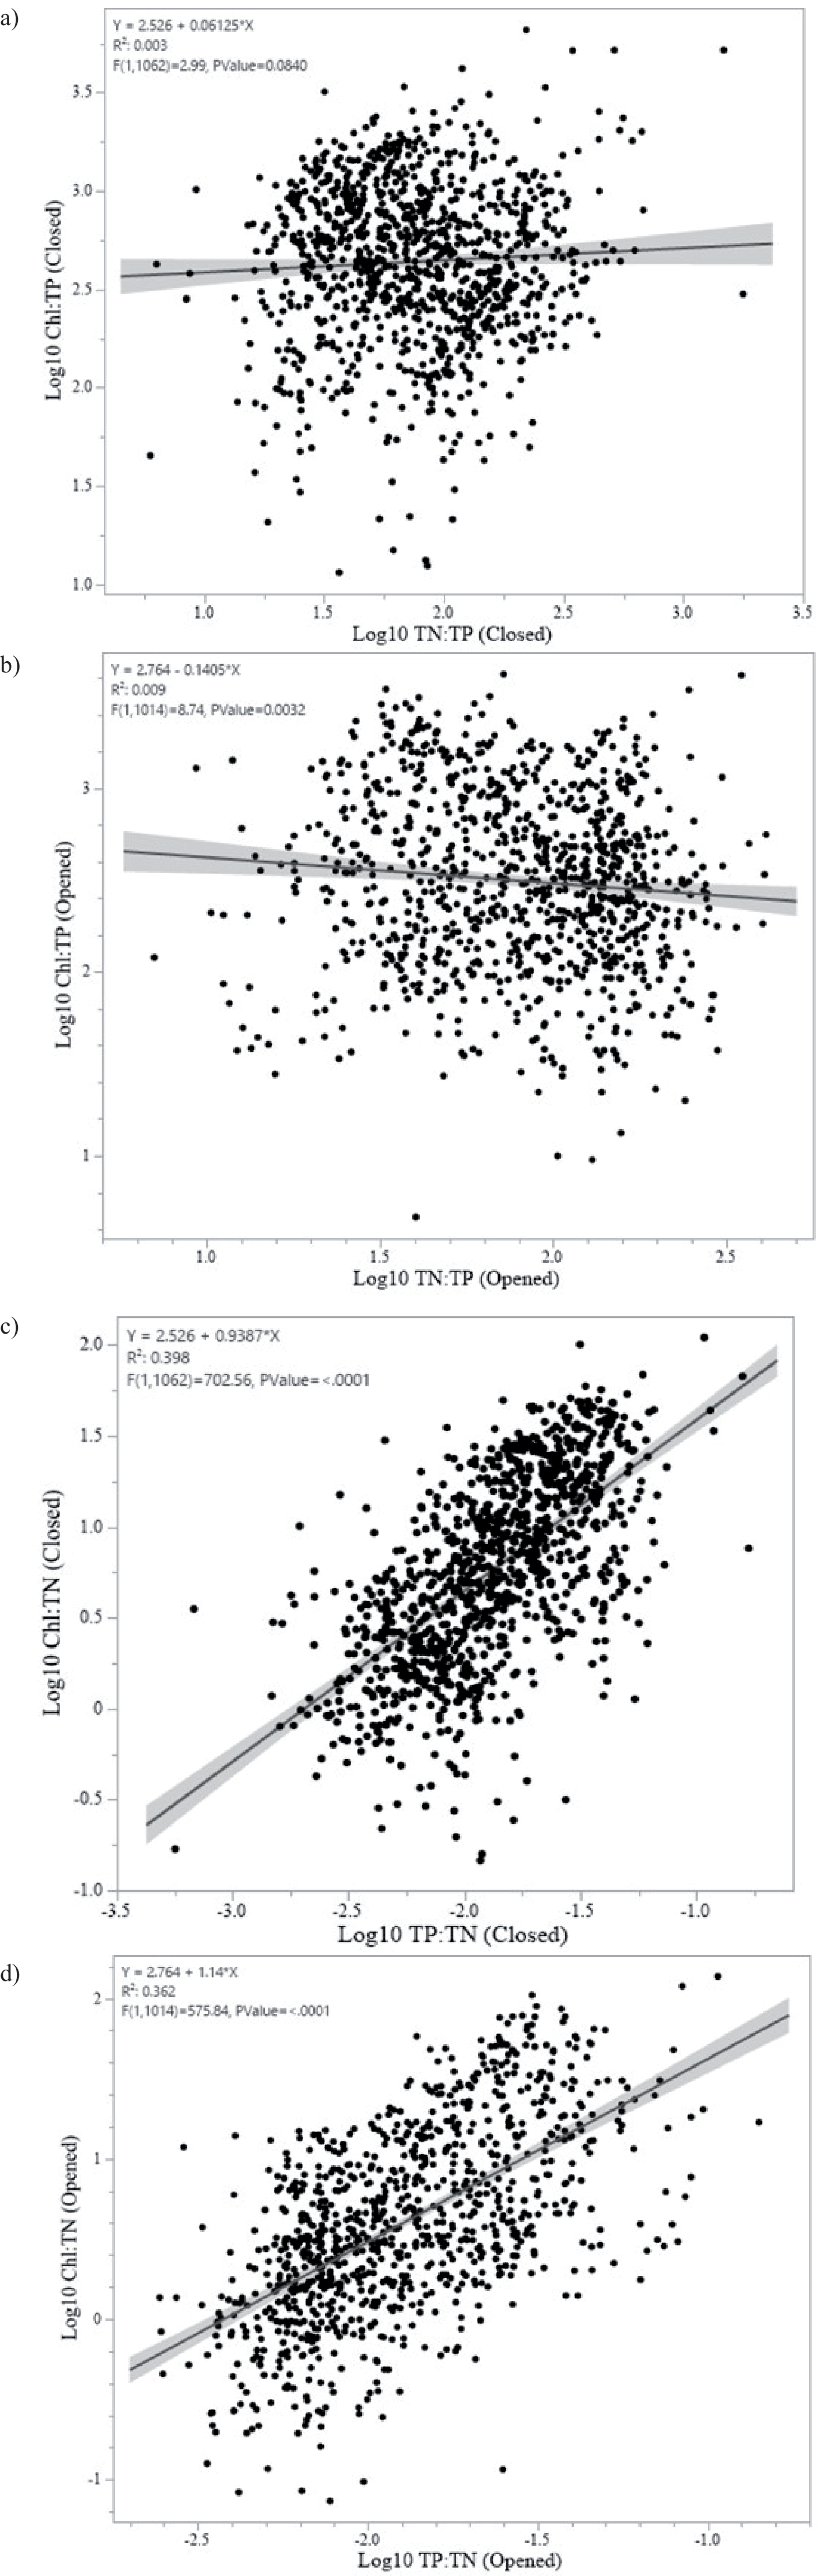
The TN:TP ratio, originated from the Redfield ratio [53], has been widely adopted to test whether a waterbody is limited by N, P, or both for aquatic primary productivity. The ratio of TN to TP concentrations (by mass) was used as an indicator of potential nutrient limitation of phytoplankton or planktonic algae, with N the only limitation if the TN:TP ratio <8 to 10, P the only limitation if the TN:TP ratio >20 to 24, and co-limitation if 9 or 10 ≤ the TN:TP ratio ≤20 to 22 [54]. Most freshwaters are likely to have more than 16 in the ratio of TN:TP, indicating that N is in oversupply [55, 56]. In this study, the TN:TP ratios of all 5 studied waterbodies were far above the Redfield ratio (16:1 by atoms, 7:1 by mass). In it, the average dam TN:TP ratio was 96, whereas the counterpart weirs was 67, indicating that P was a limiting nutrient for algal growths in both standing and flowing waters. Indeed, TN:TP ratios of most rivers and reservoirs distributed nationwide are far more than 10, indicating that a P-limited waterbody is commonly found in South Korea [57-59]. However, the TN:TP ratio may not be a good indicator or index for potential nutrient limitation and algal biomass accrual as demonstrated in other studies [60] and this study conducted in northeast Asia because there were no clear relationships between Chl:TP and TN:TP ratios during both the closed and opened periods of weir gates (Fig 8a; Fig 8b). Because the Chl:TN ratio was regressed with TP:TN ratio, for a given amount of TP, Chl a changed irrespective of the amount of TN, whereas for a given amount of TN, Chl a increased with the increasing TP as the Chl:TP ratio was regressed with the TN:TP ratio. This may imply that TP, not the TN:TP ratio, is the primary limiting factor for regulating algal abundance in the studied region.
In artificial lakes (e.g., dam reservoirs in this study), residual P in non-metabolized particles settles down and is often buried in the waterbody’s bottom sediments. In contrast, N can be lost from sedimentation processes, similarly to P in deep lakes, but it is often less efficiently removed because much more N remains in bioavailable dissolved forms [61]. In addition, denitrification is often greater in shallow waters than in deep waters and can remove up to 90% of TN inputs in shallow eutrophic lakes with short particle settling times [62]. Frequent wind-induced perturbation resuspended more P from bottom sediment surfaces into the shallow water column [63], which led to a lower TN:TP ratio in weir impoundments and the estuary dam reservoir than in the upstream dam reservoir [64]. That is, N loss and P supply from bottom sediments led to a lower TN:TP ratio in the shallow weir impoundment and the estuary dam reservoir, whereas the opposite occurred in the upstream dam reservoir that was rarely limited by bottom sediment resuspension, thus favoring a higher TN:TP ratio. Moreover, as waters moved downstream, P concentrations were elevated by an increased chance of watershed runoffs, but owing to the highest concentrations of P in the estuary dam reservoir that closed the gate most of the time during a day, the dam likely displayed a lower TN:TP ratio than the bottommost weir impoundment just above the estuary dam reservoir. High flows in general facilitated downstream movement of nutrients, thus reducing the opportunity for algal uptake in the middle-stream weir impoundments [56]. However, because of the disproportional contribution of sediment resuspension to the TN and TP ratios, downstream transport of TN was not as large as TP in quantity, presumably so that the estuary dam reservoir likely displayed a lower TN:TP ratio. Hamilton and Mitchell [65] demonstrated that wind-induced bottom resuspension in shallow lakes caused TP concentration in the water column of a waterbody increased twofold, whereas TN concentration increased by only one fifth. Therefore, care should be taken when utilizing the TN:TP ratio for determining P limitation in aquatic ecosystems. Absolute P concentration appears to be more critical than the nutrient ratio.
Fig 7.
Chl (µg L–1) and TP (mg L–1) relationships across the 5 waterbodies during the period of weir gate openings from January 2019 to December 2022 in the main stem of the Geum River (n = 1008). The gray range indicates 95 % confidence limits.
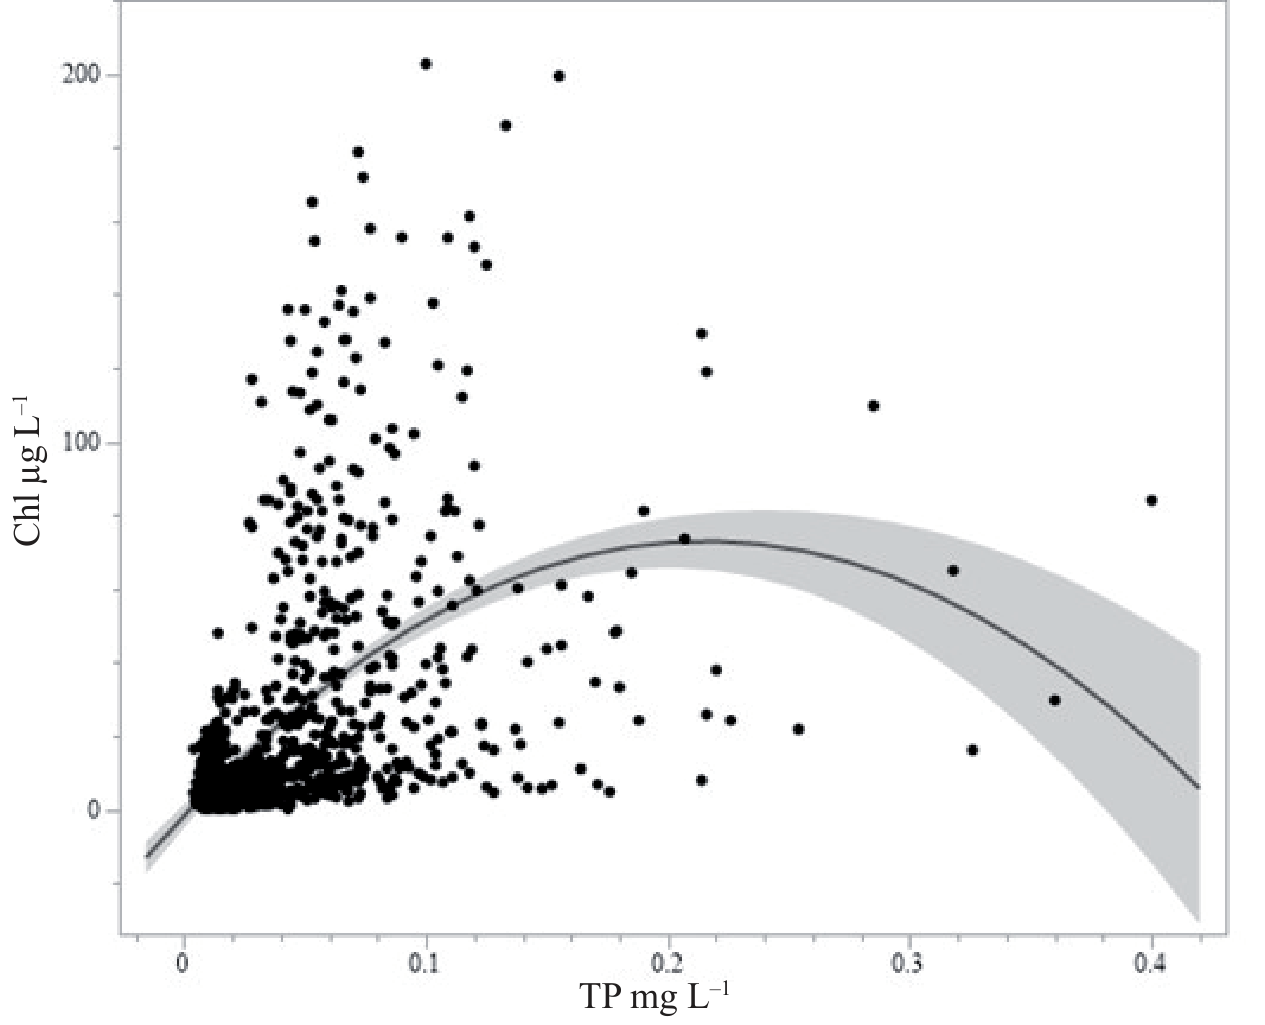
Fig 8.
Relationships a) between log10 Chl:TP and log10 TN:TP ratios (Closed) (n = 1041) and b) (Opened). The gray ranges indicate 95% confidence limits. Fig 8. Relationships c) between log10 Chl:TN and log10 TP:TN ratios (Closed) (n = 1041) (n = 1066) and d) (Opened) (n =1008). The gray ranges indicate 95% confidence limits.
Conclusions
Understanding the hydrologic and geomorphological drivers for algal limitation by nutrients is vital for controlling aquatic primary productivity and water quality management. I found that altered hydrology following weir gate openings exerted a significant influence on algal responses to water column P concentrations on a broad temporal and spatial scale. In general, this result was in agreement with other empirical studies on the effects of variation in hydrologic patterns on algal primary productivity. However, based on the observation that occurred during up to a 4-year period of full weir gate openings, my study provided a contrast to other algal biomass-P relationship studies in that the responses of algae to P became stronger and differentiated among waterbodies formed by weirs in the main stem of a river as waters moved downstream. The reflowing river following weir gate openings was large, shallow (not thermally stratified), and advantageous in utilizing interactions between nutrient-rich sediments and the water column, which provided optimum conditions for algal growth because of P supply from both external sources and internal cycling of a waterbody. Although I did not address biological factors such as the top-down grazing effect (e.g., zooplankton) in this study, it turned out that immense hydrologic forces alone could control primary productivity sufficiently to predict algal growths on a broad scale. Nonetheless, waterbodies following weir gate openings still need enough time to equilibrate with new hydrologic and topographical regimes for a prolonged time period. Geum River was dissimilar to other reflowing waterbodies in hydrologic conditions (e.g., reflooding reservoirs after prolonged drought [39]) because, unlike in their cases, there was no substantial reduction in algal biomass in water columns. Mine is perhaps the first study to quantify the effects of weir gate operation (openings) on algal primary productivity in a large human-regulated river in a temperate region of the world. My study results have offered novel insights into a hydrologic regime that intervenes in the response of algae biomass to P concentration, which is closely linked to water quality management and policy sectors. Weir gate openings were certainly a key factor limiting algal growth in eutrophication management, but they appeared to be insufficient to mitigate algal biomass accrual in a given time period, especially because of the estuary dam constructed at the mouth of the river that has operated to impound waters from upstream. To counteract the negative impacts of the man-made environments and human-induced changes on river surface water quality, prolonged and simultaneous gate openings across weir impoundments and dam reservoirs in a river’s main stem are warranted and should be monitored at a longer temporal scale.

