

Introduction
Owing to the industrial revolution, the amount of N deposited in the atmosphere has substantially increased, and the relative surplus of soil N has caused a series of ecological problems, such as soil acidification and biodiversity reduction [1]. It has indirectly caused changes in the soil P cycle by affecting the physical and chemical properties of the soil, exacerbating P restrictions, and leading to an imbalance in the N/P ratio of the soil. N and P play a key role in the biogeochemical cycle [2, 3]. They are essential mineral nutrients for plant growth and participate in plant development, playing an important role in the synthesis of plant growth proteins and genetic material [4]. Therefore, in the context of global N deposition and P deficiency, exploring the mechanism underlying the impact of N and P addition on plants’ functional traits is of great importance.
The root system enables a plant species to absorb and utilize soil resources and is an important carbon sink for terrestrial ecosystems [5]. Fine roots are root systems with a diameter ≤ 2mm, which have absorption functions and rapid turnover. They constitute important organs that absorb water and nutrients, and are an important component of energy flow and material cycle, especially the carbon cycle in terrestrial ecosystems. The roles, positions, and functions of roots vary by diameter. To date, the functions of roots have been linked to their structural levels (diameter classes). Some studies have combined root order and diameter classes to reduce workload and accurately evaluate the role of fine roots [6]. The specific root length (SRL), root diameter (RD), and root tissue density (RTD) reflect the morphological structure and function of fine roots, facilitating research on plants’ underground production strategies. Thus, the study of fine root morphology can offer insights into how fine roots adapt to their surroundings. Change in fine root morphology is influenced by external factors such as soil fertility [7, 8]. Therefore, investigating the relationship between fine root morphology and different soil environments from the perspective of root order is of great importance to the study of heterogeneity within root systems.
The diameters of the fine roots of Japanese Larix gmelinii and ChangBai Mountain broad-leafed Pinus koraiensis decrease with increasing N availability [9, 10], whereas the diameters of other tree species increase [11, 12]; Wang and Freschet found that SRL decreases with increasing of N availability in Juglans mandshurica [13, 14]. The SRL of Cunninghamia lanceolata and Cryptomeria japonica increase with N availability [15, 16]. However, the SRL of fine roots in Pinus elliottii, Phellodendron amurense, and Populus tremuloides showed no considerable response to N availability [11, 15, 17]. In contrast, relatively few studies have explored the impact of changes in P effectiveness on the morphological traits of fine roots. The SRL and RTD of Acer mono and Lespedeza bicolor considerably increased with P availability [18]. The RD and SRL of Larix gmelinii did not greatly increase after P addition [19]. N addition on trees did not exert a considerable effect on RTD [20]. In herbaceous species, RTD decreased as N and P increased [21]. The morphological characteristics of plant roots vary by species, amount of fertilization, sampling location, and soil condition. Moreover, research is mainly focused on the effects of fertilization on aboveground leaves, whereas research on the effects on underground roots remains limited. The mechanism underlying differences in the morphological characteristics of plant roots needs to be further explored.
The response characteristics of morphological traits of fine roots have been examined under different fertilization conditions. Most studies have focused on the 1–5 level root classes and used diameter as the classification standard. Research that investigated the responses of these morphological traits to fertilization in different diameter classes remains limited. In addition, the anatomical structures of herbaceous and woody species’ roots vary (i.e. the number of exodermis cells and cortical layers, and differences in xylem and lignified xylem rings) [22, 23], and the two root systems differ in adaptability of the morphological traits to fertilization. Examining the response of fine root morphological traits of plants to N and P addition not only provides insights into the adaptation strategies of the fine roots of woody and herbaceous species to nutrient addition, but also is essential for the study of plants’ functional traits varied soil heterogeneity. Thus, our study focused on 14 common green species (eight woody species and six herbaceous species) in northeast China. The morphological traits (RD, SRL, and RTD) of the different diameter classes of fine roots (R<0.5, R (0.5-1), R (1-2)) were evaluated through fertilization (N and P) experiments. Two hypotheses were proposed in this study:
(1) fine root diameter classes have different morphological plasticity to N and P addition and (2) morphological traits are positively correlated irrespective of soil nutrient availability. Addressing these questions not only contributes to the understanding of the adaptation strategies of the fine root traits of woody and herbaceous species to nutrient addition, but also has great importance for the study of regional vegetation restoration and reconstruction under conditions with soil heterogeneity.
Materials and Methods
Plant Materials
We selected eight woody species (Acer negundo L., Amorpha fruticosa L., Catalpa ovata G.Don, Cornus stolonifera Michx., Fraxinus mandschurica Rupr., Juglans mandshurica Maxim., Padus maackii (Rupr.) Kom., Sorbus alnifolia (Sieb. et Zucc.) K. Koch., and six herbaceous species (Ageratum conyzoides L., Dahlia pinnata Cav., Gazania rigens Moench., Salvia splendens Ker-Gawler., Tagetes erecta L., Zinnia elegans Jacq.). The details are shown in Table 1. The plant materials are easy-to-find seedlings, have high ornamental and applied values in urban parks and residential areas, and cover a wide range of species, including woody and herbaceous species of different life forms. The species are representative and can provide a systematic understanding of the response mechanisms and strategies of species to soil nutrient changes, as well as a theoretical basis for the cultivation and afforestation of urban and forest species.
Table 1.
List of growth form, their family, seed source, height and content of N and P additions in eight woody species and six herbaceous species.
Soil Characteristics of the Research Areas
Experimental Design and Sowing
In October 2016, we collected or purchased the plant seeds in Mudanjiang (128°02′–131°18′E, 43°24′–45°59′N), Heilongjiang province, China. At the end of March 2017, the seeds were sown in nursery pots after stratification. Plants that grew consistently were selected and transplanted into plastic pots (20 cm × 13 cm × 12 cm) (one plant per pot) at the four-leaf stage. The pot-growing substrate was a mixture of forest soil and sand (V/V 1:1) with relatively low nutrient content. Soil characteristics are shown in Table 2. Each pot contained 3 kg of air-dried soil.
Experimental Treatment
In mid-June, three nutrient addition treatments were carried out, including Control (C; 100 mL distilled water), N addition (+N; N content 0.136% (Woody), 0.116% (Herbaceous) NH4NO3 solution 100 mL), and P addition (+P; P content 0.078% (Woody), 0.071% (Herbaceous) Ca (H2PO4)2 solution 100 mL) (Table 1). Each treatment was applied to 12 pots for each species fertilization was applied 3 times at 15-day intervals. The period from fertilization to sampling lasted two months. The temperature, humidity and light intensity in the greenhouse ranged from 22.7 to 35.1°C, 31.7 to 78.0%, and 121 to 900 μmol m-2 s-1, respectively.
Research Methods
Fine Root Collection and Processing
In mid-August, we harvested all species from all species before their root systems became potbound (only a few roots of Gazania rigens Moench reached the interior wall of the nursery pots). We removed the plants from the pots and washed the roots carefully with deionized water. Afterward, the roots were kept refrigerated until analysis.
Determination of Fine Root Morphological Traits
Took out the root from the sealed bag, washed it with deionized water, and divided the roots according to the size of the RD (R<0.5, RD < 0.5 mm; R(0.5–1), 0.5mm ≤ RD ≤ 1 mm; R (1–2), 1 mm ≤ RD ≤ 2 mm) treatment [24]. Ac (Ageratum conyzoides L.), Te (Tagetes erecta L.), As (Acer saccharum L.), and Cs (Cornus stolonifera Michx.) have thinner root systems and have not grown a root diameter class of 1–2 mm. After dividing the roots, we placed them in a porcelain plate filled with deionized water and used a root image scanner (Epson 700) to scan to obtain a fine root image. The scanned fine roots are then placed in an envelope and dried (65℃, 24 hours) to weigh the dry weight to the nearest 0.0001 g. Fine root images were measured using Win-RHIZO2008a (Regent Instruments Canada Inc.) software to determine the average diameter, total length, total volume, and other parameters of each diameter class. The calculation formula for SRL and RTD is as follows:
SRL (m·g-1) = root length (m) / root dry weight (g);
RTD (g·cm-3) = root dry weight (g) / volume (cm3).
Data Analyses
The mean value and standard error of RD, SRL, and RTD for each diameter class of each plant species under control, N addition, and P addition, as well as the mean value and standard error of various indicators for herbaceous and woody species were calculated (each species serves as a repeat) with SPSS software (2010, V. 19.0, SPSS Inc., Cary, NC, USA). If results met the hypothesis, a Duncan post-hoc test was used to determine significant differences among means, otherwise, a Dunnett,s T3 post-hoc test was used to determine significant differences among means. We used three-way factorial ANOVA to test the influence of N addition on each species, and P addition on each species, separately, as well as their interactions with root morphological traits. The mean values of each species with three treatments were used. We used R2 in the regression analysis. Origin software was used for graphical representation.
Results
We found that the application of N and P fertilizers significantly affected RD, SRL, and RTD, and species, diameter classes, and the interactions of species and diameter classes all affected RD, SRL, and RTD at a highly significant level, whereas the three interactions were only significant for SRL (Table 3).
Table 3.
Three-way analysis of variance (ANOVA) for the effects of plant species, diameter classes, and fertilization on root morphological traits.
Table 4.
Effects of N and P addition on the SRL, RD and RTD of different diameter classes of 14 species and woody and herbaceous species.
[i] Ac: Ageratum conyzoides L.; Dp: Dahlia pinnata Cav.;Gr:Gazania rigens Moench.; Ss: Salvia splendens Ker-Gawler.; Te: Tagetes erecta L.; Ze: Zinnia elegans Jacq.; AS: Acer saccharum L.; Af: Amorpha fruticosa L.; Co: Catalpa ovate G.Don; Cs: Cornus stolonifera Michx.; Fm: Fraxinus mandshurica Rupr.; Jm: Juglans mandshurica Maxim.; Pm: Padus maackii Kom; Sa: Sorbus alnifolia K. Koch. Different letters indicated significant (P<0.05) differences among individual species under the N and P addition treatments compared with the control, respectively.
Effects of N and P Addition on the SRL of 14 Plant Species
The SRL of all diameter classes increased in most herbaceous species after N and P addition, and decreased in woody species at R<0.5 (except Sa), with significant differences in SRL after N additions only in Af and Co, and at R(0.5–1) and R(1–2) for all species (except N additions in Af and Pm and P additions in Co, Fm, Jm, and Pm). At R<0.5, N addition significantly reduced the SRL of Af and Co (woody species), with a rate of change of 27–41% (Table 4). At R(0.5-1), N addition significantly increased the SRL of Ss and Ze (herbaceous species), with a rate of change of 55–86% (Table 4). At R(1-2), N addition significantly increased the SRL of Sa (woody species) by 36% (Table 4). P addition significantly increased the SRL of Te (herbaceous species) at R<0.5 by 41%, while the differences at other diameter classes were not significant.
Effects of N and P Addition on the RD of 14 Plant Species
N and P addition increased the RD of all diameter classes of roots in most species. N and P addition significantly increased the RD of Sa (woody species) at R<0.5, with a rate of change of 9% and 7%, respectively (Table 4). The effects of N and P addition were not significant for all species at R(0.5–1). N addition significantly increased the RD of Ze (herbaceous species) with a rate of change of 23%, and P addition significantly increased the RD of Co (woody species) with a rate of change of 17% at R(1–2) (Table 4).
Effects of N and P Addition on the RTD of 14 Plant Species
N and P addition had inconsistent effects on the RTD of herbaceous and woody species at different diameter classes. At R<0.5, N and P addition had inconsistent effects on the RTD of different species, but none of them showed significant differences (Table 4). N addition significantly reduced the RTD of Ze (herbaceous species), Af, and Co (woody species) by 15–44% at R(0.5–1), and N addition significantly increased the RTD of Pm (woody species) by 40%. P addition significantly reduced Af and Cs (woody species) by 16–24% (Table 4). At R(1–2), N and P addition significantly increased the RTD of Ss (herbaceous species) with a rate of change of 27–30%, whereas the woody species responded significantly to N addition only in Co and Jm with an increase of 18–33% (Table 4).
Effects of N and P Addition on Morphological Traits of Woody and Herbaceous Species
The SRL of herbaceous species was 66% greater than that of woody species at R<0.5. N addition had a significant effect on woody species, and resulted in reducing the SRL of woody species by 28% ((Table 4); the RD of woody species was greater than that of herbs by 20%, and N addition significantly increased the RD of woody species by 9%, and P addition increased the RD of woody species by 4% ((Table 4); the RTD of woody species was greater than that of herbs by 20%, and N and P addition significantly reduce the SRL of herbs by 22% and 30%, respectively. At R(0.5–1), the SRL of herbaceous species was 122% larger than that of woody species, and the application of N fertilizer had a significant effect on the SRL of herbs, which increased by 46%; the RD of woody species was 2% larger than that of herbaceous species; and the RTD of woody species was 74% larger than that of herbaceous species (Table 4); at R(1–2), the SRL of herbaceous species was 154% greater than woody species at R(1–2); the RD of woody species was 30% greater than that of herbs; and RTD was 89% greater than that of herbs (Table 4).
Effects of N and P Addition on the Interactions Among Morphological Traits of 14 Plant Species
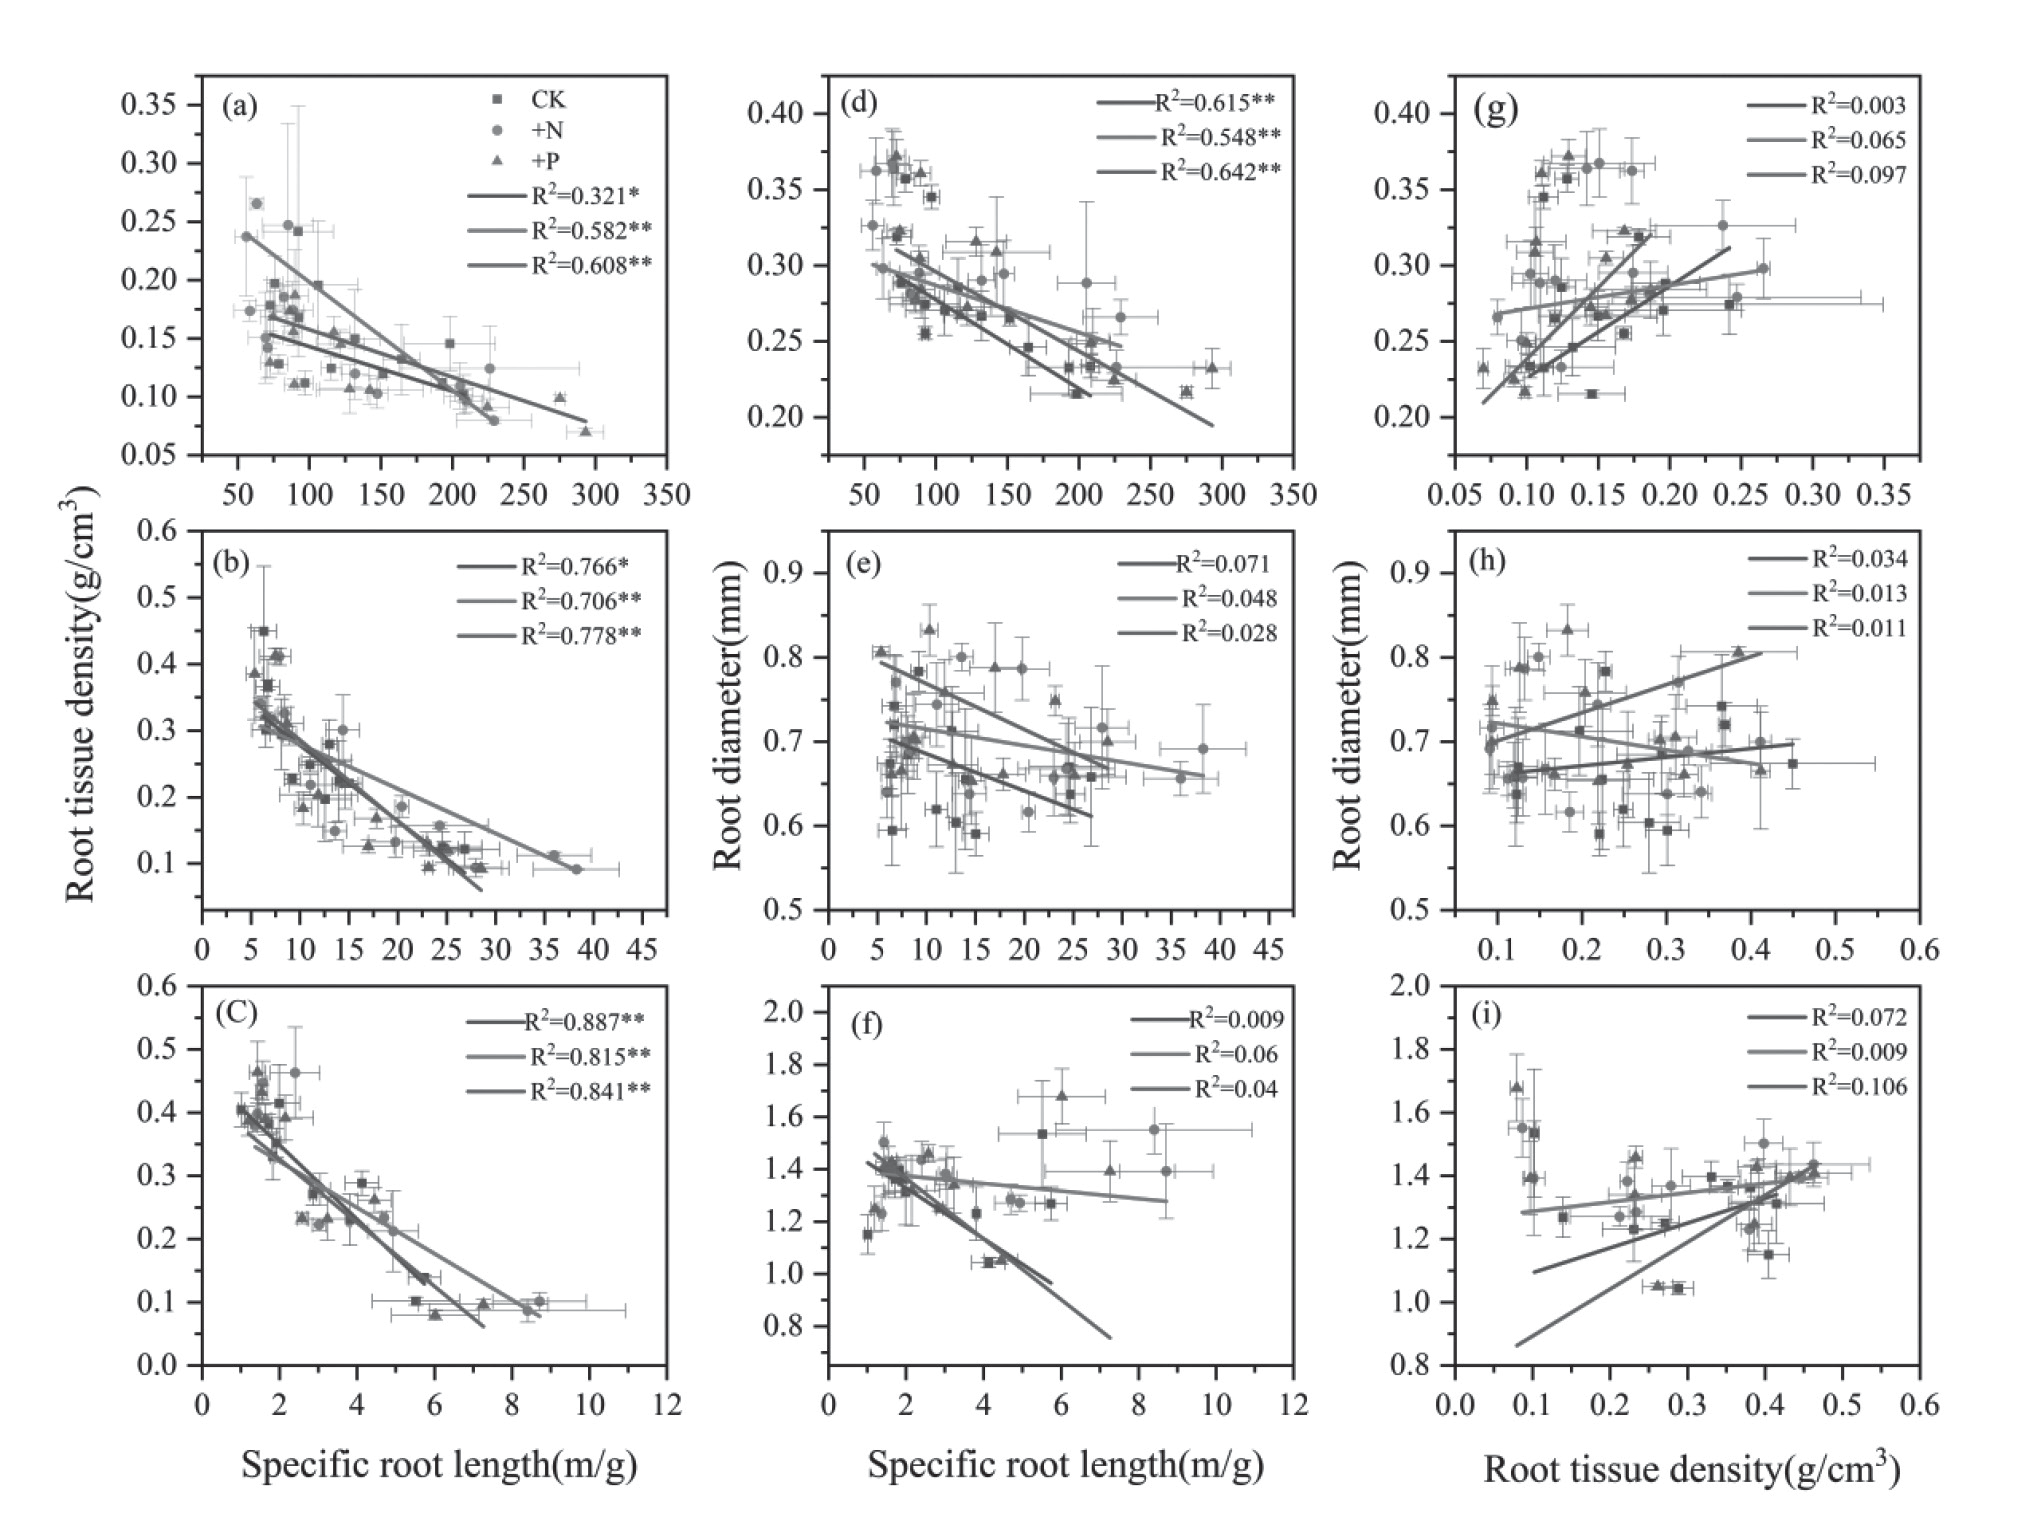
In this study, The SRL and RTD had a significant negative correlation, and this relationship was not altered by diameter classes and fertilizer application (Fig. 1a, b, c). When no fertilizer was applied, SRL explained 32.1%, 76.6%, and 88.7% of the variation in RTD at different diameter classes, respectively, and the higher the diameter class, the higher the rate of variation in RTD explained by SRL; after N and P addition, SRL explained 58.2% and 60.8% of the variation in RTD at diameter class of R<0.5, respectively (Fig. 1a); after P addition, the negative correlation between SRL and RTD was more obvious at R(0.5–1) (Fig. 1b, c).
As can be seen from Fig. 1d, e, f, SRL, and RD had negative correlations at different diameter classes, regardless of fertilizer application. SRL and RD were significantly negatively correlated only at R<0.5, with SRL explaining 61.5% of the variation in RD, while N and P addition did not change their negative correlation, explaining 54.8% and 64.2% of the variation in RD, respectively (Fig. 1d). In the other two diameter classes, SRL explained less of the variation in RD, between 1.0 and 7.1% (Fig. 1e, f). As shown in Fig. 1g, h, i, the relationship between RTD and RD was not significant at different diameter classes, regardless of fertilizer application.
Discussion
The RD, SRL, and RTD are important root morphological indicators. SRL can reflect a plant’s ability to obtain soil nutrients. The absorption capacities of fine roots increase with their SRL [25, 26]. Diameter not only reflects the growth and development of species, but also reflects the functional level of fine roots [27]. The RTD of fine roots represents the investment of root biomass per unit of root length [28]. Exploring the response of plant roots’ morphological traits to fertilization can reflect various plant construction strategies [29, 30]. In this study, after Note: a, R<0.5, C:R2 = 0.321**, +N:R2 = 0.582**, +P:R2 = 0.608**; b, R(0.5-1), C:R2 = 0.766**, +N:R2 = 0.706**, +P:R2 = 0.778**; c, R(1-2), C:R2 = 0.887**, +N:R2 = 0.815**, +P:R2 = 0.841**; d, R<0.5, C:R2 = 0.615**, +N:R2 = 0.548**, +P:R2 = 0.642**; e, R(0.5-1), C:R2 = 0.071, +N:R2 = 0.048, +P:R2 = 0.028; f, R(1-2), C:R2 = 0.009, +N:R2 = 0.06, +P:R2 = 0.04; g, R<0.5, C:R2 = 0.003, +N:R2 = 0.065, +P:R2 = 0.097; h, R(0.5-1), C:R2 = 0.034, +N:R2 = 0.013, +P:R2 = 0.011; i,R(1-2), C:R2 = 0.072, +N:R2 = 0.009, +P:R2 = 0.106. the addition of N and P, the RD, SRL, and RTD of fine roots at each diameter class of the 14 species showed different trends. The magnitude and difference in changes in various traits varied by species, diameter class, and plant type, confirming our first hypothesis.
Fig. 1.
Relationships between the RD, SRL, and RTD of different diameter classes. Control (CK, black box), N addition (+N, red circle), and P addition (+P, blue triangle).
Effects of N and P Addition on Root Morphological Traits of Different Diameter Classes in Species
After N and P addition, the SRL of each diameter class of herbaceous species increased, reflecting enhanced water and nutrient absorption capacity. Differences in Ss and Te were significant only when N was added to the diameter class at R (0.5–1) and P was added to the diameter class at R<0.5. Wurzburger and Wright recorded the responses of fine roots to long-term N, P, and K fertilization in the Panama lowland tropical forest [31]. The results demonstrated that the addition of P reduced the densities of the fine roots and increased their SRL, which is consistent with our results. In addition, Zhan showed that Leymus chinensis absorbed high amounts of nutrient resources at medium N levels, and adapted to increased nutrient concentrations by reducing its SRL [32]. This result is different from the results of our study, indicating that the adaptability of herbaceous species to N addition is the same in roots with different diameter classes. However, a high amount of N fertilizer affects a plant’s absorption capacity. After N addition, the SRL of woody species decreased at R<0.5 (except Sa), and significant differences were observed only in Af and Co. However, the SRL of each species at R(0.5–1) and R(1–2) diameter classes increased (except Pm and Af) (Table 4), and the changes in the SRL of eight species with roots of different diameter classes were not significant after P addition. After N and P addition, the SRL of herbs at all classes and most woody species at R(0.5–1) and R(1–2) diameter classes increased. The corresponding cortical thickness, number of cortical layers, and diameter of cortical cells decreased, and thus, the rate of nutrient absorption increased [33].
In this study, most roots grew at the end of the root system at R<0.5 and mainly played the role of absorbing roots [34]. Their root system absorbed high amounts of water and nutrients, but the absorption capacities of the root system decreased with increasing thickness of the root system. The plant root system was limited by nutrients, thus showing a considerable increase in SRL.N application greatly increased the proliferation rate of fine roots of Castanopsis fabri, nutrient absorption was achieved by increasing the SRL [35], which is similar to the Co. Changes in the SRL of woody species at R<0.5 after N addition may be due to the increase in cortex thickness or stele diameter, which led to a decrease in absorption capacity. The results of Zhou showed that low N levels increased the cortical thickness of the 1st~3rd fine roots of Korean pine [36], supporting our conclusion.
After N addition, the variation trend of SRL in the fine roots of the woody species varied among diameter classes, The possible reasons were that soil nutrients already met the needs of woody species roots, and the increase in N availability led to a decrease in SRL in the roots with high absorption and transportation capacities. It showed reduced root metabolism and prolonged lifespan [37], and thus did not need to produce roots with fine RD and high SRL. In all the species, the addition of N and P increased the RD, which was not affected by the diameter class, and considerably affected only the RD at R<0.5 (Co), and R (1–2) (Sa and Ze) (P < 0.05) (Table 4). This result was different from that of Zhang [38], who studied nine tree species fertilized for two years in North America and showed that N fertilizer treatment had no considerable effect on fine root diameter at different root order levels. A study of five subalpine forest types showed that the diameters of fine roots did not markedly change along the soil fertility gradient [39]. However, Wen found that the application of P on Zea mays L. resulted in a decrease in RD [40], and Beroueg’s study showed the same effect [41]. These results demonstrated the close relationship between root morphological traits and anatomical traits, that is, the positive correlation of diameter and cortical thickness with stele diameter. Cortical structure may affect the absorption capacities of fine roots. The thinner the cortex, the shorter the distance of nutrient absorption to the vascular transport site, the faster the absorption rate, and the thicker the cortex, the slower the absorption rate [42]. The results of this study illustrated that Sa and Ze have a strategy that prolongs lifespan after N addition.
The data showed that the addition of N and P resulted in an increase in RD in most species. This increase is an adaptation strategy developed by species to accelerate root water and nutrient turnover. N addition can lower soil pH, and a significant increase in Al ions in the soil can lead to toxicity and RD thickening [43]. However, plant roots do not tend to change their own morphological characteristics to adapt to changes in soil environments and nutrient content, and they adapt to environmental changes by regulating biomass [17], metabolic level [44], and turnover [45]. Different tree species have different foraging strategies for soil nutrient resources. The addition of N reduced the RTD of the fine roots in various diameter classes of herbaceous species, and the trend of changes in woody species was inconsistent. Substantial differences were observed only in the R(0.5–1) and R(1–2) diameter classes. At R<0.5, N addition reduced the RTD of nine species, and P addition reduced the RTD of 11 species, but the difference was not significant. Compared with higher root diameter classes, the lower roots of these species showed poor stress resistance, vigorous metabolism, strong absorption ability, and fast growth rate. This result was consistent with the research of An. The root growth rates of species with low RTD were higher than those of species with high RTD [46]. At R(0.5–1), fertilization markedly reduced the RTD of Ze, Af, Co, and Cs, whereas N application greatly increased the RTD of Pm. At R(1–2), N application increased the RTD of six species, and the RTD of Ss, Co, and Jm greatly increased. The addition of N and P considerably increased the RTD of Ss. As the root diameter class increased, plants preferentially built defense and stress resistance to resist risks. With the increase of diameter class, the RTD of most species increased, and the RTD was related to the number of xylem vessels, the proportion of the cell wall of the stele or stele, and the number of ventilated tissues. The number of xylem vessel of species decreased with RTD, the proportion of the cell wall of the stele or stele decreased, and the absorption capacity was enhanced. However, the number of xylem vessels of species with enhanced RTD increased, and the number of ventilated tissues and the corresponding absorption capacity decreased, showing the basic strategy of plants to prolong their lifespan after N addition [31]. Our conclusions were supported by the study of Li [47], who studied eight species of the Fagaceae family, and demonstrated that absorbing roots were transformed into transporting roots, SRL decreased, and RTD increased as the root diameter increased.
Yang showed that on the morphological traits of the fine roots of shrubs under subalpine forests in western Sichuan were similar [48]. The growth rate and lifespan of fine roots were influenced by RTD. Our data showed that different fertilization treatments had different effects on the RTD at different root diameter classes, and changes in species were not considerable. Therefore, we were unable to determine the degree of influence on fine roots’ lifespan and growth rate through the effects of fertilization on RTD. The roots’ morphological traits at different diameter classes exhibited inconsistent responses to fertilization. The reason may be that RD differ by species, and diameter classes may contain several functional levels of root orders. Different root orders have different strategies for nutrient absorption and utilization [48].
Differences in the Effects of N and P Addition on Morphological Traits of the Roots of Herbaceous and Woody Species
The SRL of herbaceous species was significantly higher than that of woody species and was not affected by fertilization. This result is consistent with the results of Freschet [49], who showed that herbaceous species absorb water and nutrients. Plants with large SRL have a greater advantage over plants with small SRL by investing lower amounts of C in root construction [26], but the turnover rate is fast and the roots have reduced lifespan. Fertilization increased the RD of woody and herbaceous species, and woody species had higher RD than herbs. Herbs had thinner roots and decomposed more slowly than woody plants [50]. These differences might be attributable to the particular anatomy characterized by a high proportion of recalcitrant tissues, such as xylem and lignified xylem rings, whose cell walls are mainly composed of cellulose and hemicellulose [50]. These characteristics of woody species may inhibit root turnover and increase lifespan. However, at R(1-2), the RD of herbaceous species was larger than that of woody species after N addition, probably because of the increase in soil N effectiveness. The root system changed its strategy of obtaining water and nutrients externally, and prolonged the lifespan by increasing the RD in order to obtain more nutrients [51]. The RTD of woody species was always greater than that of herbaceous species and was not affected by fertilization. Fertilization had little effect on the overall herbaceous and woody species as the root diameter increased. This result is inconsistent with the studies of Beidler [52], possibly because of interspecific differences in fertilization methods. The decrease in the RTD of herbaceous and woody species after N and P fertilizer treatments as root diameter increased indicated that the defense system of the root systems was basically complete, and a high degree of lignification occurred, which was not greatly affected by the fertilization treatments.
Effect of N and P Addition on the Correlation Among Roots’ Morphological Traits
Under a condition with environmental heterogeneity, plant roots’ functional traits do not exist in isolation, and are closely linked, thus ensuring survival and reproduction. Plants do not respond to changes in their surroundings by changing a single trait. They undergo a series of trade-offs and synergistic changes in traits. This pattern is common in plant communities and ecosystems [53]. The SRL is strongly correlated with RD and RTD [54], which reflect root construction strategies and are considerably correlated with root absorptive capacity and longevity [55].
In woodland habitats with fertile soils, plants obtain resources with low biomass by preferentially increasing SRL and RD [56]. In this study, the SRL and RD were significantly negatively correlated only at R<0.5, consistent with the study of Li [47]. SRL and RD can reach a trade-off relationship in low-grade roots. N and P addition did not change this negative correlation, suggesting that this change is a general pattern of plant adaptation to a habitat, and confirming our second hypothesis. At R(1-2), RD and RTD increasing with diameter was a response to plant adaptation to nutrient changes [34]. Ostonen found that only 1/4 of the dataset of fine roots of 12 different species from Europe showed a significant correlation between RD and RTD [57]. Xiong showed no significant correlation for class 2–4 roots, but discovered a clear trade-off between RD and RTD for the lowest fine roots; they suggested that the lowest roots may be limited by carbohydrate availability [58]. Our data suggested that the relationship between RTD and RD was not significant regardless of fertilization. We need to collect data from larger samples for in-depth analyses.
Our result showed that SRL and RTD had a significant negative correlation, consistent with the studies of Zadworny [55], Sun [56] and Zhuo [59]. This relationship reflects a nutrient uptake strategy of plants [60]. As the diameter increased, the coefficient of variation in RTD increased, and the significance of the negative correlation increased. The low-level roots mainly absorbed nutrient and water and had a fast metabolic rate. The fine roots were built with small inputs, thus having a large SRL and small RTD. By contrast, the high-level roots were lignified and mainly used for transport and storage, and had a large RD and RTD. Root defense was enhanced by increase in RTD. Fertilizer application increased the changes in RTD and SRL; Secondly, fertilizer application led to a significant decrease in soil pH, subjecting the root system to stress [34, 61, 62], which inhibited the root elongation, and affected the root morphology. Wang found no negative correlation between SRL and RTD [13], and Kramer-Walterand found that variation in SRL was complex and variable [63]. This variation was constrained by roots’ morphological characteristics, such as root length and RD, RTD was one of the factors affecting the SRL, and its linkage with the SRL was unclear. The relationship between SRL and RTD was diversified because of species differences and environmental factors.
Conclusions
The morphological traits of root systems with different diameters of 14 common green species (eight woody and six herbaceous) in northeast China were explored: 1) N and P addition greatly affected the RD, SRL, and RTD, and the effects of tree species, diameter class and relationships of tree species and diameter class with RD, SRL, and RTD were highly significant. The SRL of herbaceous species were significantly higher than those of woody species, reflecting the tendency of herbs to increase water and nutrient acquisition capacity by increasing SRL. This characteristic enhances their competitive advantage over woody species, which preferentially develop root defense. The RTD was consistently greater than that of herbaceous species, independent of fertilizer application. 2) Correlations among root traits were found among the diameter classes, and N and P addition did not change the negative correlation between SRL and RD. However, fertilization increased the significance of the negative correlation between SRL and RTD. This result suggested that plants make a trade-off between growth and defense by changing root traits, and that the effects of fertilization on the correlation of traits varied. This study reveals the differences in root traits and correlations among the traits of 14 greening plants of different diameter classes in northeast China, offering insights into the ecological strategies of the root systems of the 14 species, and provides theoretical references regarding the structures and functions of ecosystems in northeast China.

