

Introduction
The nutrient elements in plants primarily originate from the soil, and fertilization stands out as one of the most effective methods to enhance soil nutrients. Nitrogen (N) and phosphorus (P) play crucial roles as essential nutrients for plant elongation and growth, offering material support for the survival and development of plants [1]. Research has demonstrated that the addition of nutrients, including N and P, can effectively contribute to the restoration of soil productivity [2].
The root system of plants is a crucial component responsible for water transport within the plant and the absorption and utilization of soil nutrients. In previous studies, the criterion for categorizing fine roots has often been a root diameter of < 2mm [3], emphasizing their primary function of nutrient absorption. Over the course of long-term evolution, fine roots exhibit a remarkable ability to adapt to the underground environment, optimizing their ecological resource acquisition through self-adjustment [4]. As the most dynamic part of the plant root system, fine roots display more pronounced responses to changes in soil conditions [5] and exhibit improved effects following the addition of exogenous nutrients. Fine roots actively absorb nutrients from the soil to provide plants with essential nutrients and water. The presence of significant heterogeneity among different diameter classes results in variations in the chemical composition of fine roots [6]. The carbon (C) and N content in plant fine roots play a crucial role in maintaining nutrient cycling and energy flow in the entire ecosystem [7]. Investigating the content of C and N as well as the carbon-to-nitrogen ratio (C/N) in plant root systems is beneficial for exploring nutrient allocation within plants and the nutrient transport relationship between soil and plant bodies [8]. Previous studies have revealed a close correlation between plant root functions and root order [9]. Furthermore, past research has shown that, influenced by structural heterogeneity, the chemical composition and response to fertilization vary among fine roots with different diameters within 2mm [3, 10]. However, such differences in various plant functional types and under different nutrient additions have not been reported in the existing literature.
Nitrogen, a vital component of various compounds like proteins and nucleic acids, plays a crucial role in plant physiology [11]. On the other hand, carbon is an essential element for the diverse physiological and biochemical reactions within plants. The C/N reflects the plant's growth rate [12], highlighting the necessity of studying the composition and content of C and N in plants. In recent years, both domestic and international scholars have mainly focused on studying the relationships between C, N, and P in plant leaves and roots. There has been relatively less research on the variation of chemical traits in plant fine roots of different diameter classes after fertilization, particularly concerning the impact of increased soil phosphorus availability on the C and N chemical characteristics of plant fine roots.
Considering the differences in life history between woody and herbaceous plants, as well as the heterogeneity in the structure of roots with different diameters, this study focuses on 8 species of woody plants and 6 species of herbaceous plants used in afforestation and landscaping projects in the northeastern region of China. Through the application of exogenous N and P fertilizers, the research measures the content of C and N, C/N, within different root class diameters (including root diameters of less than 0.5 mm (R<0.5); root diameters of 0.5-1 mm (R (0.5-1)); root diameters of 1-2 mm (R (1-2)). The aim is to explore the responses of C and N chemical traits in fine roots of different diameter classes from species with different life forms to changes in soil nutrients. The study attempts to investigate the following aspects: 1) whether there are similar trends in the chemical traits of fine roots with different diameters for woody and herbaceous plants under nitrogen and phosphorus addition, 2) whether the response to fertilization is more pronounced in fine roots with a diameter of R<0.5, and 3) whether fertilization alters the relationships between C and N chemical traits. Analyzing these aspects not only helps uncover the relationships between changes in soil nutrients and the nutrient absorption and utilization strategies of plant fine roots with different diameters but also holds significant implications for understanding the adaptive strategies of plants with different life forms to nutrient addition. The results of this study can provide a scientific basis for understanding the nutrient absorption and utilization strategies of herbaceous and woody plant fine roots and their response mechanisms to changes in soil N and P.
Materials and Methods
Plant Materials
The Institute chose 8 woody plants and 6 herbaceous plants commonly employed in urban landscape green space systems and afforestation projects in the northeastern region of China. These plants belong to 9 families and 14 genera, and their characteristics are detailed in Table 1. The selection of these 14 plant species is based on their frequent use, ease of accessibility, and exceptional ornamental and practical value. Additionally, the chosen plant species exhibit comprehensive coverage, representing various life forms, including both woody and herbaceous types. This diversity makes the study on the chemical characteristics of fine roots C and N in seedlings somewhat representative.
Experimental Design and Sowing
In October 2016, we collected or purchased the plant seeds in Mudanjiang (128°02′–131°18′E, 43°24′– 45°59′N), Heilongjiang province, China. In March 2017, the seedling’s seeds after germination treatment were sown in the seedling tray. When plant seedlings grew more than four true leaves, plants with consistent growth were selected from each provenance and colonized into plastic pots (20 cm*13 cm*12 cm), one plant per pot. The pot-growing substrate was a mixture of forest soil and sand (v/v 1:1) with relatively low nutrient content.
Table 1.
List of growth forms, their family, seed source, height and content of N and P additions in eight woody species and six herbaceous species.
Soil Characteristics of the Research Areas
Mudanjiang Location
Each pot contained 3 kg of air-dried soil. Soil characteristics: pH: 6.81 ± 0.07; Total C: 21.88 ± 0.17 (g•kg-1); Total N: 2.77 ± 0.02 (g•kg-1); Total P: 0.48 ± 0.02 (g•kg-1); Total K: 29.33 ± 0.19 (g•kg-1); Available N: 67.43 ± 2.54 (mg•kg-1); Available P: 50.65 ± 0.23 (mg•kg-1); Available K: 55.15 ± 0.26 (mg•kg-1); Cation exchange capacity: 10.17 ± 0.02 (cmol•kg-1); Base Saturation: 70.26 ± 0.001 (%).
Experimental Treatment
The fertilization treatment was carried out in mid-June. In order to ensure the smooth progress of this experiment, the preliminary test was carried out before this, so as to determine the content of nitrogen fertilizer and phosphate fertilizer used in the experiment. Three fertilization treatments were set up in this experiment, including Control (C; 100 mL distilled water), N addition (+N; N content 0.136% (Woody), 0.116% (Herbaceous) NH4NO3 solution 100 mL), and P addition (+P; P content 0.078% (Woody), 0.071% (Herbaceous) Ca (H2PO4)2 solution 100 mL). Fertilization was applied 3 times at 15 days intervals. The period from fertilization to sampling lasted two months.
Research Methods
Fine Root Collection and Processing
During the test, the temperature, humidity, and light intensity in the greenhouse ranged from 22.7 to 35.1°C, 31.7 to 78.0%, and 121 to 900 μmol m-2 s-1, respectively, and the normal maintenance management procedure was carried out. At the end of the experiment, the root system was collected by excavation method, the plants in the pot were taken out, the crushed soil around the root system was carefully removed, and the soil particles remaining on the root system were carefully washed with deionized water to absorb the water. The roots were put into a sealed bag and sealed in the refrigerator for freezing and storing for C and N chemical trait analysis.
Determination of Fine Root C and N Chemical Traits
Took out the root from the sealed bag, washed it with deionized water, and divided the roots according to the size of the root diameter, (including root diameters of less than 0.5 mm (R<0.5, 14 species); root diameters of 0.5-1 mm (R (0.5-1), 14 species); root diameters of 1-2 mm (R (1-2)), 10 species) treatment [13], Ac (Ageratum conyzoides L., Te (Tagetes erecta L.),, As (Acer saccharum L.) and Cs (Cornus stolonifera Michx.), they have thinner root systems and have not grown a root diameter class of 1-2mm. After dividing the roots, the fine roots are placed in a 65℃ bake-out furnace for drying, then ground and screened through 100 mesh. The root total carbon concentration (RTC) and root total nitrogen concentration (RTN) in the fine root samples are measured using an elemental analyzer (Vario MACRO, Elementar F Analysensysteme, Germany). The calculation formula for the root carbon to nitrogen ratio (RC/N) is as follows:
RC/N= Root total C concentration/
Data Analyses
We used SPSS 19.0 for statistical analysis, and Origin software was employed for graphical representation. Mean values and standard errors for RTC, RTN, and RC/N within three diameter classes were calculated for each plant sample under control, nitrogen addition, and phosphorus addition conditions. Additionally, mean values and standard errors for various indicators were calculated for herbaceous and woody species, with each species treated as a replicate. To assess significance, one-way ANOVA and Duncan's method were utilized for the analysis of variance and multiple comparisons, respectively. The impact of species, diameter class, and fertilization on the C and N chemical characteristics of plant roots, along with their interactions, were examined through a three-way factorial ANOVA.
Results
The study revealed that species, diameter class, and the interaction between species and diameter class all reached highly significant levels of impact on RTN, RTC, and RC/N. However, the interaction of the three factors was only highly significant in influencing the RC/N (Table 2).
Effects of N and P Addition on the RTC of 14 Plant Species
After N and P addition treatments, the trends in RTC varied inconsistently across species and diameter classes compared to the control. In the R<0.5, among herbaceous plants, only the RTC in the Ss significantly decreased by 10.44% after N addition, while the woody plant Cs significantly increased by 9.55%. No significant responses to phosphorus addition were observed in any species (Table 3). In the R (0.5-1), among herbaceous plants, only Ze exhibited a significant increase of 2.68% after N addition, while among woody plants, Af and Co significantly increased by 1.03% and 2.97%, respectively. After P addition, there were no significant differences observed in herbaceous and woody plants compared to the control, with variation ranges of -3.92% to 0.68% and -2.25% to 1.01%, respectively (Table 3). In the R(1-2), among herbaceous plants, both Cs and Ze exhibited significant changes compared to the control after N addition, with the highest increase being 11.71%. Among woody plants, the difference was significant in Co, with variation ranges for all species being -1.13% to 3.57% (Table 3). After P addition, only Cs showed a significant increase of 13.45%, while the RTC in woody plants did not significantly decrease, with a reduction range of 0.18% to 2.27% (Table 3).
Table 2.
Three-way analysis of variance (ANOVA) for the effects of plant species, diameter classes and fertilization on root morphological traits.
Effects of N and P Addition on the RTN of 14 Plant Species
After N addition, the RTN in the fine roots of both herbaceous and woody plants increased across all diameter classes. Except for the R<0.5 in Dp and R (1-2) in Ss, the RTN in all diameter classes of each species was significantly different compared to the control. In the R<0.5, the increase ranged from 19.15% to 63.29% for herbaceous plants and from 55.79% to 150.45% for woody plants (Table 3). In the R (0.5-1), the increase ranged from 38.53% to 147.74% for herbaceous plants and from 93.68% to 290.97% for woody plants (Table 3). In the R(1-2), the increase ranged from 46.51% to 232.68% for herbaceous plants and from 128.89% to 293.15% for woody plants (Table 3).
In this study, the response of RTN to P addition varied across each species and diameter class. Only Te in the R<0.5, Af in the R (0.5-1), and Gr and Af in the R (1-2) roots showed a significant difference in RTN compared to the control, with inconsistent trends among species.
Effects of N and P Addition on the RC/N of 14 Plant Species
After N addition, the RC/N in the fine roots of both herbaceous and woody plants decreased in all diameter classes compared to the control. Except for Dp in the R<0.5, Ss in R (0.5-1), and R (1-2), the RC/N in all diameter classes of other species showed significant changes. Among herbaceous plants across the three diameter classes, Gr exhibited the most substantial reduction in RC/N, with decreases of -38.23%, -59.21%, and -69.31%. Among woody plants, Jm showed the most significant difference in RC/N compared to the control, with reductions of -60.91%, -74.14%, and -74.5% (Table 3).
After P addition, the response trends in RC/N varied across species and diameter classes. In the R<0.5, among herbaceous plants, only Te significantly increased by 28.09%, while among woody plants, Fm significantly increased by 10.98%, and Af significantly decreased by 11.55% (Table 3). In the R (0.5-1), among herbaceous plants, Gr significantly decreased by 31.16%, while among woody plants, Fm significantly increased by 8.69%, and Af, Co, and Jm significantly decreased, with Af showing the highest reduction of 25.1% (Table 3). In the R (1-2), the RC/N in fine roots decreased for herbaceous plants, with Gr showing a significant difference from the control, with a reduction of 30.91%. Among woody plants, only Af showed a significant change in root C/N, with a variation range of -33.28% to 20.43% (Table 3).
Effects of N and P Addition on C and N Chemical Traits of Woody and Herbaceous Species
In the control group, the RTN and RTC in woody plants were higher than those in herbaceous plants across all diameter classes (Table 3). In R<0.5, R (0.5-1), and R (1- 2), woody plants exhibited higher RTC than herbaceous plants by 2.46%, 1.58%, and 5.45%, respectively. The RTN was higher in woody plants by 23.33%, 29.9%, and 45.76%, respectively (Table 3). However, the RC/N was higher in herbaceous plants, with herbaceous plants showing RC/N higher than woody plants by 21.19%, 40.12%, and 55.74% across the three diameter classes. After N addition, both herbaceous and woody plants exhibited significant changes in RTN across all diameter classes. While the RTC of herbaceous and woody plants at three diameter classes increased or decreased, they were not significantly different from the control. RTN increased by 36.4%, 69.92%, and 119.21% for herbaceous plants and 82.5%, 164.59%, and 180.47% for woody plants across the three diameter classes (Table 3). The RC/N significantly decreased in woody plants, with reductions of 45.43%, 63.72%, and 65.55% in R<0.5, R (0.5-1) and R (1-2), respectively (Table 3). In herbaceous plants, the RC/N significantly decreased only in R<0.5 compared to the control. After P addition, there were no significant effects on RTN, RTC, and RC/N across the three diameter classes.
The Relationship and Effects of N and P Addition on the Interactions Among C and N Chemical Traits in Roots of 14 Plant Species
Among the various diameter classes of the 14 plant species, there exists a certain relationship between the root C and N chemical characteristics. Under both control and fertilization treatments, a highly significant negative correlation was observed between RTN and RC/N across all diameter classes (Table 4).
PCA revealed a negative correlation between RTN and RC/N across different diameter classes in each treatment. When R<0.5, RTC and RTN showed a positive correlation in all treatments, with a negative correlation between RTC and RC/N in the control group and N addition. After P addition, there was a weak negative correlation between RTC with RC/N. The cumulative explanation of the first and second principal component axes accounted for 82.1% of the variation in root chemical traits between the control group and N and P added plants in R<0.5 (Fig. 1a). In the R (0.5-1), a weak negative correlation between RTC and RTN was observed in the control group and after P addition, while a positive correlation emerged after N addition. A weak positive correlation was observed between RTC and RC/N in the control group, and a weak negative correlation was observed after N and P addition. The cumulative explanation of the first and second principal component axes accounted for 84.1% of the variation in root chemical traits between the control group and N and P added plants in R (0.5-1) (Fig. 1b). When R (1-2), there was a weak negative correlation between RTC and RTN in the control group, while after N and P addition, RTC and RTN were both positively correlated. In the control group and after P addition, there was a weak positive correlation between RTC and RC/N, while after N addition, a negative correlation emerged between RTC and RC/N. The cumulative explanation of the first and second principal component axes accounted for 75.7% of the variation in root chemical traits between the control group and N and P added plants in R (1-2) (Fig. 1c).
Table 3.
Effects of N and P addition on the RTC, RTN, and RC/N of different diameter classes of 14 species and woody and herbaceous species.
[i] Note: Ac: Ageratum conyzoides L.; Dp: Dahlia pinnata Cav.;Gr: Gazania rigens Moench.; Ss: Salvia splendens Ker-Gawler.; Te: Tagetes erecta L.; Ze: Zinnia elegans Jacq.; AS: Acer saccharum L.; Af: Amorpha fruticosa L.; Co: Catalpa ovate G.Don; Cs: Cornus stolonifera Michx.; Fm: Fraxinus mandshurica Rupr.; Jm: Juglans mandshurica Maxim.; Pm: Padus maackii Kom; Sa: Sorbus alnifolia K. Koch. Different letters indicated significant (P<0.05) differences among individual species under the N and P addition treatments compared with the control, respectively.
Table 4.
Correlation of C and N chemical traits in 14 plants under each treatment.
Discussion
In this study, after N and P addition, the RTC, RTN, and RC/N of fine roots in 14 plant species exhibited different changes across diameter classes. The chemical characteristics of roots C and N showed significant differences due to variations in diameter class, species, and life form.
Fig.1.
Principal component analysis (PCA) for Different Different Diameter RTC; RTN and RC/N in 14 plants grown under Nitrogen and Phosphorus addition. a: R<0.5; b: R (0.5-1); c: R (1-2). Ac: Ageratum conyzoides L.; Dp: Dahlia pinnata Cav.;Gr: Gazania rigens Moench.; Ss: Salvia splendens Ker-Gawler.; Te: Tagetes erecta L.; Ze: Zinnia elegans Jacq.; AS: Acer saccharum L.; Af: Amorpha fruticosa L.; Co: Catalpa ovate G.Don; Cs: Cornus stolonifera Michx.; Fm: Fraxinus mandshurica Rupr.; Jm: Juglans mandshurica Maxim.; Pm: Padus maackii Kom; Sa: Sorbus alnifolia K. Koch. Different letters indicated significant (P<0.05) differences among individual species under the N and P addition treatments compared with the control, respectively. The Root C; N chemical traits are shown in blue. RTN-CK:Root total N concentration in the control; RTN-N+:Root total N concentration in the Nitrogen addition; RTN-P+:Root total N concentration in the Phosphorus addition; RTC-CK:Root total C concentration in the control; RTC-N+:Root total C concentration in the Nitrogen addition; RTC-P+:Root total C concentration in the Phosphorus addition; RC/N-CK:RC/N in the control; RC/N-N+:RC/N in the Nitrogen addition; RC/N-P+:RC/N in the Phosphorus.
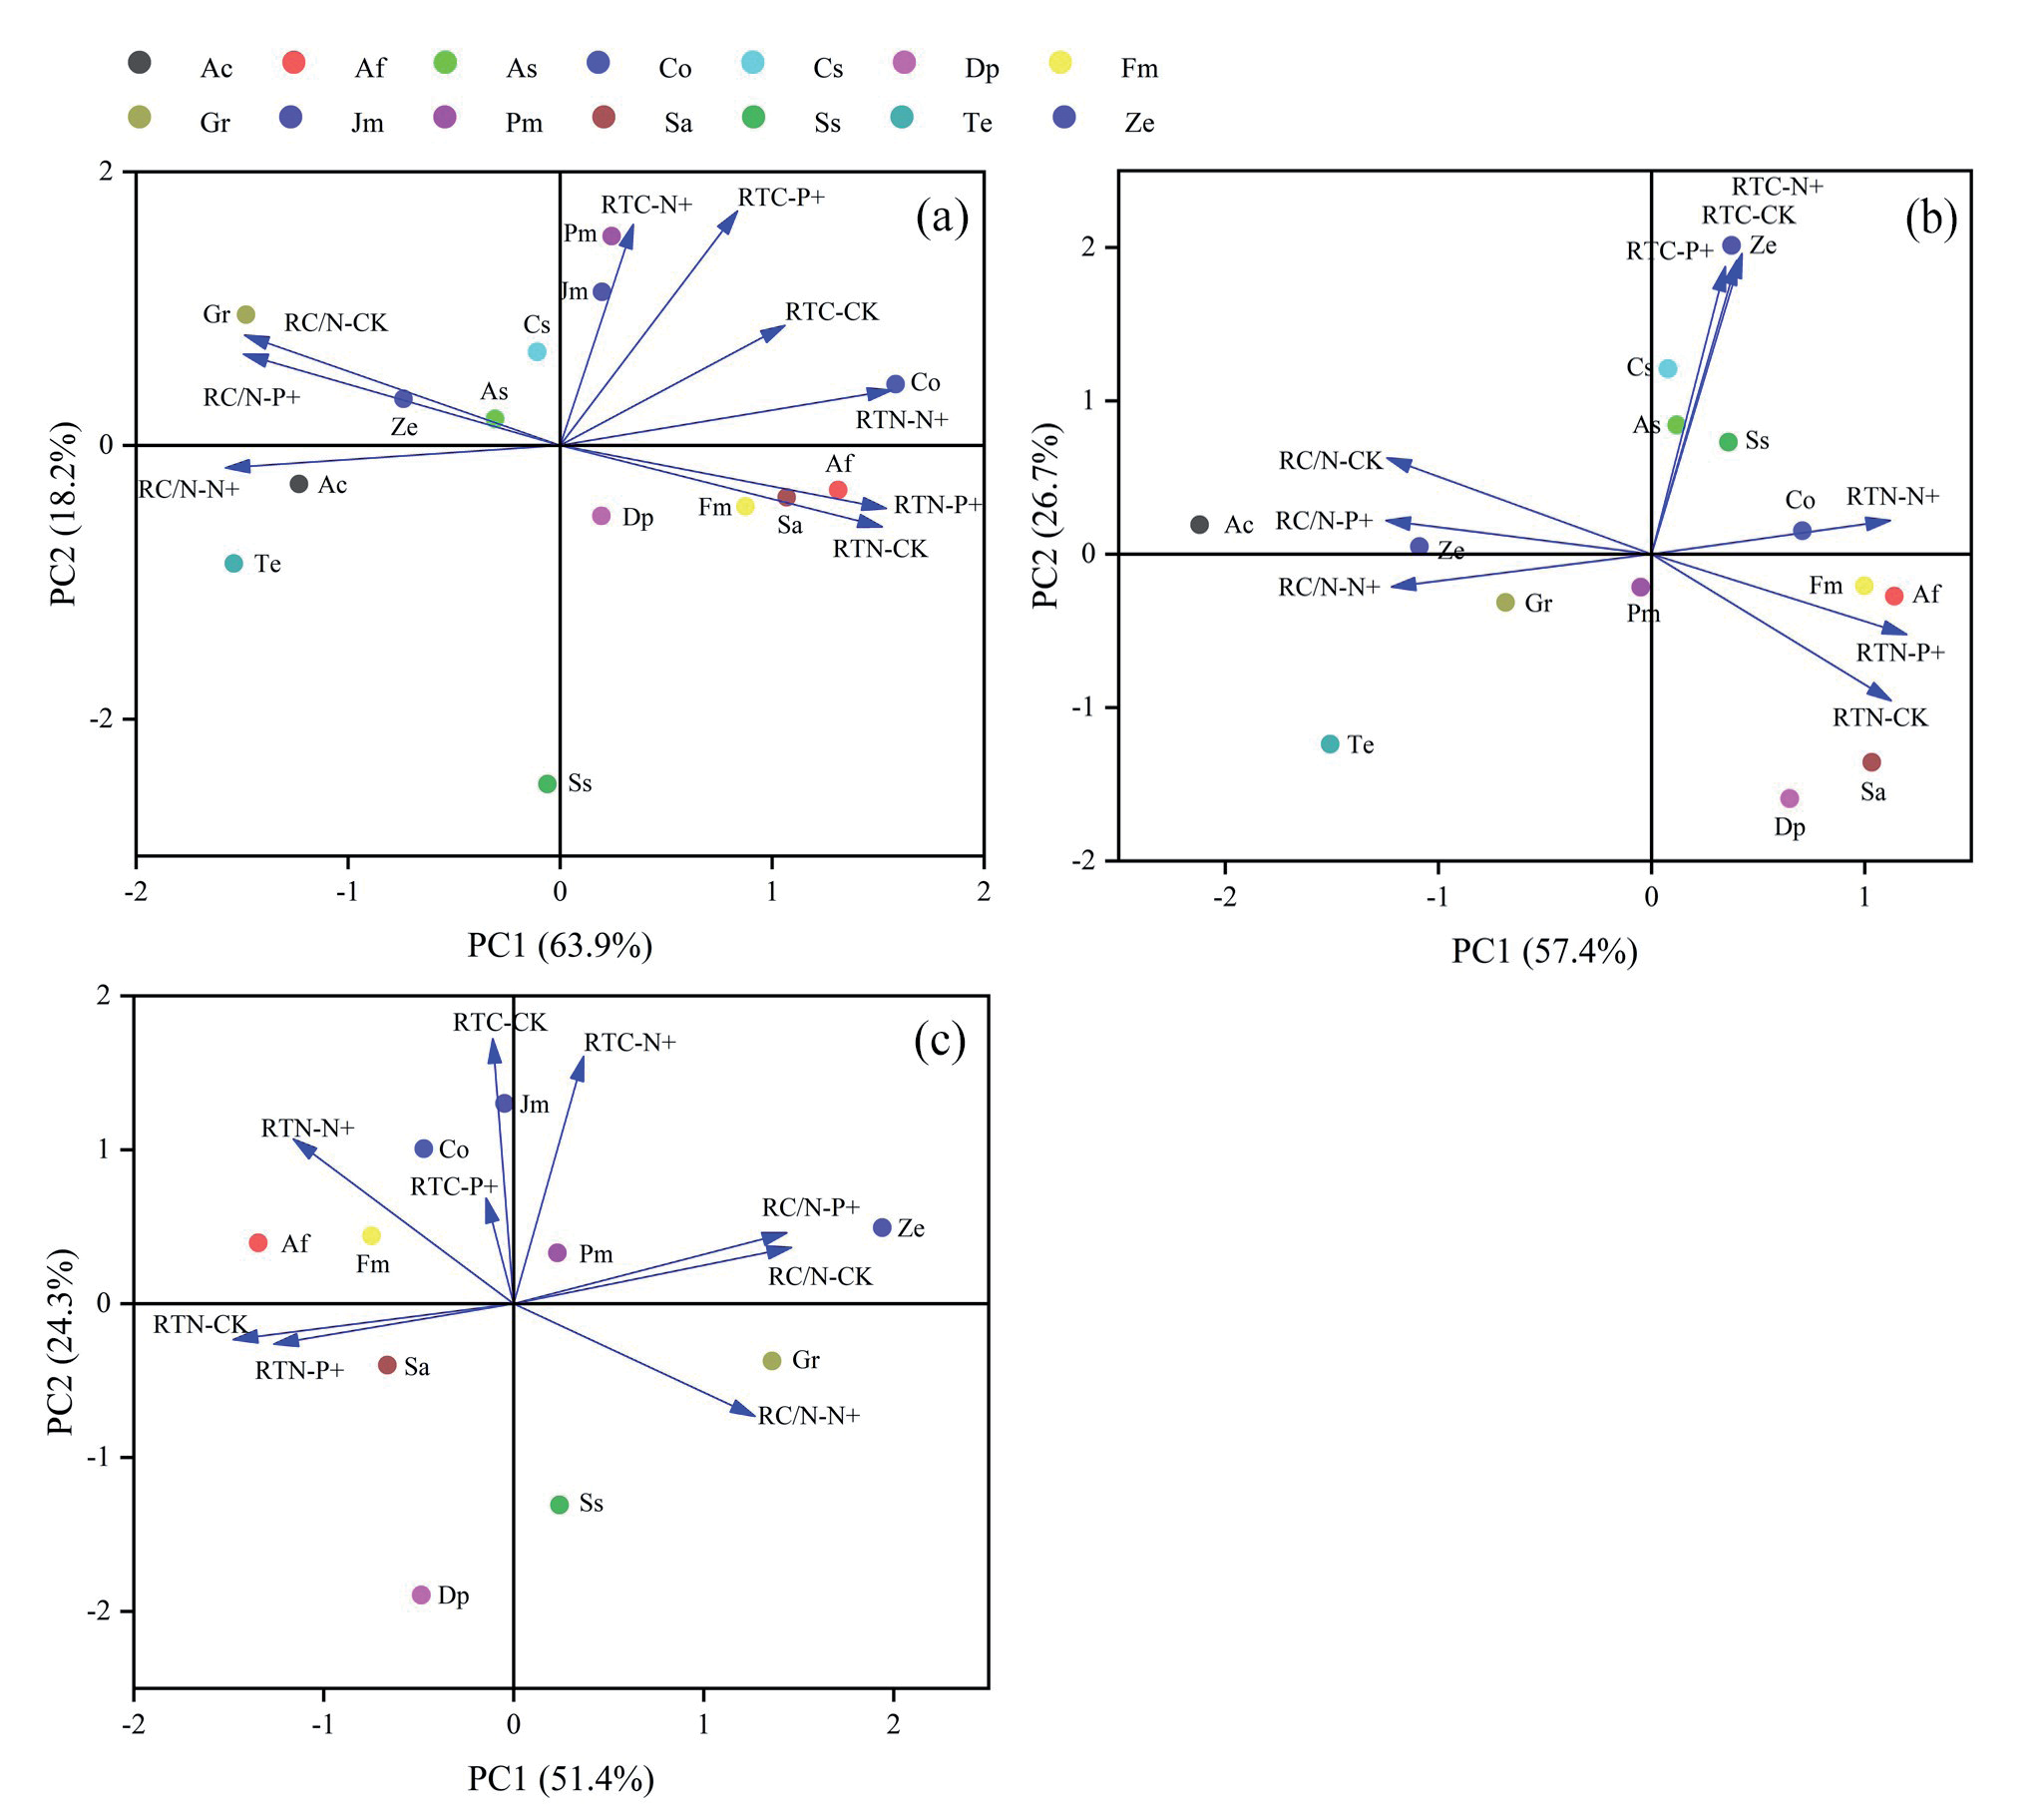
Effects of N and P Addition on C and N Chemical Traits of Different Diameter Classes of Root in Species
For plants, N and P are indispensable nutrients in their growth and development processes, and the demand for these elements is substantial. If the demand cannot be met, plants will adapt to the environmental conditions by reducing their growth rate. External nutrient addition is an effective method to address this phenomenon. After N and P addition, the RTC of fine roots in 14 plant species showed varying trends and changes across diameter classes. Previous studies, such as Yu et al., found a slight increase in carbon concentration in 1-5 grade roots of Larix kaempferi (Lamb.) Carr after N fertilization with no significant difference [14]. Another study indicated a decrease in carbon concentration in fine roots (<2mm) after N addition [15], consistent with the results of this experiment.
After N addition, the RTC of the R<0.5 diameter class in the species Ss significantly decreased. Research has shown that N fertilization leads to a significant increase in total N concentration in Ss leaves, resulting in an excessive carbon cost [16]. Following N addition, only the RTC of the R<0.5 diameter class in the Cs significantly increased. For the R (0.5-1), the RTC of Ze, Af, and Co, as well as the R (1-2) of Ss, Ze, and Co, all showed a significant increase. Previous studies have found that in the R (0-1) diameter class of Larix gmelinii (Ruprecht) Kuzeneva, RTC is the smallest [17]. This is because larger roots in this diameter range primarily function in nutrient transport and storage, exhibiting strong lignification, and require sufficient carbon to maintain root morphological structure [18].
After P addition, only the RTC of the R (1-2) in Ss significantly increased. Studies have indicated that after P addition, the total C concentration in the first-order roots of Ss significantly decreased [15]. Wang et al. found that the C content of first-order roots is related to their leaf growth habits and life forms [19]. This may be the reason for the significant increase in the RTC of Ss after P fertilization. Wang et al. discovered that N and P additions have no significant impact on the root carbon content of 4 plant species in Hulunbuir grassland [20]. Similar results were observed for Populus tremuloides Michx. [21], Cunninghamia lanceolata (Lamb) Hook. [22], and Larix kaempferi (Lamb) Carr. [23], where fine root carbon content increased after fertilization, consistent with the findings of this experiment. Different plant species exhibit variations in the response of RTC to N and P addition. One possible reason is the variability among species, leading to different nutrient requirements. Another reason is that, for many species, RTC shows an insignificant response to fertilization, possibly because carbon serves as the framework for constructing mineral nutrients in plant bodies and is a structural substance with strong stability, less influenced by external factors [24]. Additionally, N, as a necessary nutrient for plant growth, needs to be obtained from the soil, while C mainly originates from the photosynthetic carbon cycle [25]. This might be one of the reasons why RTC shows an insignificant response to N and P fertilizer addition.
After N addition, the RTN of all species and diameter classes increased. Studies have suggested that the absorption capacity of plant roots for N is related to the soil nitrogen availability [26]. The increase in nitrate nitrogen content in the soil after N fertilization is more favorable for the absorption of nitrogen by fine roots [27]. In this study, the differences were significant for all species and diameter classes, except for the herbaceous plant R<0.5 of Dp and the R (1-2) of Ss. Research has shown that with an increase in N content in the soil, the RTN in the fine roots of Cunninghamia lanceolata [28], Larix gmelinii [29], and Abies fabri (mast.) Craib [30] increases, consistent with the findings of this experiment. Zhou et al. found that N addition increases soil nitrogen availability, leading to a significant increase in the RTN of 1-5 order roots of Pinus koraiensis [9]. Studies by Yu et al. have shown that N addition can effectively alleviate N deficiency in fine roots (<2mm) of Alhagi sparsifolia Shap [31]. This is because, after N addition, fine roots of various diameter classes respond, and the RTN significantly increases compared to the natural environment. This may be attributed to the fact that fine roots, as the most active part of the root system, can better absorb and store nitrogen to increase their nitrogen content when soil nitrogen availability increases after N addition. Another study suggested a decline in nitrogen content in the fine roots of Pleioblastus amarus after several years of N addition [32], which is inconsistent with the results of this experiment. The differences could be due to variations in environmental conditions and species.
After P addition, only the herbaceous plant Te in the R<0.5 exhibited a significant decrease in RTN, and the woody plant Af in the R (0.5-1), the herbaceous plant Gr, and the woody plant Af in the R (1-2) showed a significant increase in RTN. The remaining species showed no significant differences. Studies have indicated that P fertilizer has no significant impact on C content in roots [33]. Research by He et al. found an increase in N content in fine roots (<2mm) of Fm after P addition [34]. Bai suggested a decrease of 9.07% in the RTN of Larix principis-rupprechtii Mayr after P addition compared to the natural environment, which is generally consistent with our study [35]. This variation may be attributed to the different abilities of plants belonging to different species and life forms in absorbing soil nutrients through their root systems [15]. After P addition, the RTN in the R<0.5 of leguminous plant Af showed no significant difference, while differences were significant in the R (0.5-1) and R (1-2). With increasing diameter class, the nitrogen-fixing efficiency of the root system improved, leading to a significant increase in RTN. Augusto et al. [36] and Maistry et al. [37] proposed an increase in biological nitrogen fixation rates of leguminous plants after P addition. Some studies have suggested that due to the unique nitrogen-fixing ability of leguminous plants, P addition enhances their ability to absorb P fertilizer without being influenced by soil nitrogen deficiency, making them more advantageous in terms of N accumulation [38, 39], supporting our research findings.
The RC/N can reflect the plant's ability to absorb and utilize soil nutrients and assimilate carbon within a certain range [40]. After N addition, the RC/N of all 14 plant species in each diameter class decreased. Except for the herbaceous plant Dp in the R<0.5 and the herbaceous plant Ss in the R (0.5-1) and R (1-2), the RC/N in other species and diameter classes showed significant differences. An increase in soil nitrogen content significantly decreased the RC/N of plants [41]. Research has indicated that due to differences in C and N sources and functions, C is generally considered to have a minor impact on plant growth, while changes in nitrogen content are the main influencing factors for the C/N [42]. Zhou et al. found a significant reduction in the RC/N of Pinus koraiensis fine roots (1-5 order roots) after N fertilizer application [9]. They explained this change as an increase in soil nitrogen content, which enhanced soil nitrogen availability, thereby accelerating the rate of fine root respiration. With the increase in RTN, the RC/N decreased. These findings support our conclusions. After P addition, the RC/N of the woody plant Af significantly decreased in all diameter classes. This may be attributed to P addition promoting the plant root biomass and carbohydrate accumulation of leguminous plants, thereby enhancing their biological nitrogen fixation rates [43, 44]. Nitrogen fixation provides a supply of nitrogen in the soil, and the increased nitrogen absorbed by fine roots significantly reduces their RC/N. In the woody plant Fm, the RC/N significantly increased in the R<0.5 and R (0.5-1). This is consistent with the research findings of Zhang on Fm, where the RC/N increased after P fertilizer application [45]. This is because P addition affects the fine root's nitrogen absorption capacity and promotes the efficiency of nitrogen utilization in plant fine roots [46].
Differences in the Effects of N and P Addition on Root C and N Chemical Traits of Herbaceous and Woody Species
This study indicates that under N and P addition, the average RTC and RTN of woody plants are higher than those of herbaceous plants. Zhang et al. found in a study on different life forms of plants in Hainan that woody plants generally have higher C and N concentrations in their root systems compared to herbaceous plants [47]. This difference may be attributed to variations in their life histories, leading to differences in the fine root's ability to absorb soil nutrients [48]. After N addition, the RTN of herbaceous and woody plants at each diameter class changed significantly. The RC/N of woody plants significantly decreased in all diameter classes compared to the control, while herbaceous plants showed significant differences only in the R<0.5 diameter class. This is likely because of the increased nitrogen in the soil leading to the accumulation of N in fine roots. Research by Hao on woody plants such as Quercus acutissima and Liquidambar formosana found that N addition significantly reduced the RC/N [49], supporting the results of this study. Studies have shown that a decrease in the RC/N has a positive effect on the decomposition of fine roots by microorganisms after plant senescence and contributes to their nutrient cycling [50], supporting the importance of exogenous nutrients N and P addition to plants. After fertilization, the difference in RTC between woody and herbaceous plants increased in the R<0.5 compared to the control, but decreased or remained unchanged in the R (0.5-1) and R (1-2). This is consistent with previous conclusions, indicating differences in nutrient allocation among fine roots of different diameter classes [51]. After N and P addition, the average RC/N of woody and herbaceous plants at each diameter class exhibited an opposite relationship to RTC and RTN. This may be because most of the N in the plant is absorbed by fine roots from the soil, while C is mostly assimilated through photosynthesis [52]. Additionally, as a structural substance in plants, C is less affected by external factors such as fertilization. Therefore, changes in the RC/N after fertilization are mainly related to the RTN. Different plant life forms have varying degrees of root development, leading to differences in the extent of nutrient absorption and utilization from the soil. In this study, after N and P addition, the average RTN of woody plants was higher than that of herbaceous plants at each diameter class, resulting in a relatively larger average RC/N for herbaceous plants across all diameter classes.
Effect of N and P Addition on the Correlation among Root C and N Chemical Traits
In the process of plant growth, N often acts as a limiting factor for its development, and the process of plants absorbing N from the soil may impact the fixation and storage of C within them. Moreover, in the metabolic processes of plants, a significant amount of protein enzymes (N libraries) is required for carbon fixation. Studying the relationship between C and N traits in different diameter classes of fine roots is beneficial for understanding the nutrient absorption capacity of plant fine roots at various diameter classes and the distribution strategy of C. In the control group, there is a positive correlation between RTC and RTN when the diameter is less than R<0.5. However, for R (0.5-1) and R (1-2), the correlation between RTC and RTN is not significant. This is because fine roots in lower diameter classes are more active, with faster metabolic processes and strong respiratory capabilities, requiring a substantial amount of N to support enzyme synthesis [53]. The process of absorbing nitrogen from the soil by fine roots in lower diameter classes consumes a large amount of C as an energy source [54]. With the increase in diameter class, RTN significantly decreases, while the variation in RTC is not obvious, showing instances of increase, decrease, or no change. This is consistent with previous research results [55, 56]. As the diameter class increases, the root system transitions from absorbing roots to transporting roots. Transporting roots, as the main organs for storing and transporting nutrients, use stored nutrients for the growth of above-ground organs of trees during the suitable growing season, leading to a decrease in N content.
The study indicates that, regardless of fertilization, there is a significant negative correlation between the RTN and RC/N at different root diameter classes for various plant species. Research by Sun et al. on the C and N stoichiometry of different root types in China found a highly significant negative correlation between RTN and RC/N [57]. This is because C serves as the fundamental structure of the plant body and does not impose restrictive effects on plant growth, with the primary influence on C/N being attributed to changes in N levels. Studies have shown that fertilization significantly increases C and N concentrations in fine roots, while the RC/N significantly decreases [44]. After P addition, the RTN of Schima superba significantly decreases, and there is a pronounced negative correlation between RC/N and RTN [24]. This suggests that although fertilization alters nutrient levels in the soil, leading to changes in RTC and RTN, it does not change the relationship between RTN and RC/N, with N remaining the primary factor influencing C/N.
Conclusions
Through the study of 14 plants (8 woody plants and 6 herbaceous plants) widely planted in landscaping and afforestation in the northeastern region of China and analyzing the effects of N and P fertilization on the chemical characteristics of fine roots at different diameter classes, the following findings were observed:
1) N and P fertilization significantly influenced the RTN and RC/N. The effects on the chemical characteristics of roots reached a highly significant level, involving interactions between species, diameter classes, and the combination of species and diameter classes. Herbaceous plants exhibited higher RC/N compared to woody plants. N fertilization significantly increased the RTN for both herbaceous and woody plants at various diameter classes. For woody plants, the RC/N significantly decreased, indicating different nutrient absorption, utilization capabilities, and accumulation strategies between woody and herbaceous plant roots.
2) In the control, there was a positive correlation between RTC and RTN when the root diameter was R<0.5. However, this correlation was not significant at R(0.5-1) and R(1-2), suggesting that the functional roles and metabolic capabilities of fine roots at different diameter classes are related. Regardless of fertilization, there was always a significant negative correlation between RTN and RC/N at all diameter classes. This indicates that although fertilization alters the effectiveness of soil N and P, causing changes in C and N concentrations inside fine roots, C, as a structural substance, is more stable than N. Therefore, the RC/N is primarily influenced by changes in RTN. This study delves into the responses of different diameter classes of chemical characteristics of fine roots, specifically C and N traits, in 14 plant species in the northeastern region of China to N and P additions. The exploration of the correlations between these traits contributes to understanding the allocation and adaptation strategies exhibited by fine roots of different plant species in response to changes in soil nutrient conditions caused by fertilization.

