

Introduction
Toxic element pollution in the soil is a serious global environmental problem [1]. Long-term exposure to toxic elements in air, water, and soil not only affects plant growth and development but also causes oxidative damage in plants [2, 3]. It can also have serious consequences on human health, leading to abnormal growth and development, cancer, and mental retardation [4–6]. Mining is an important source of heavy metal pollution. Phytoremediation is an effective solution for addressing toxic element pollution in soil. It can be widely used in various contaminated areas, significantly reducing management costs and improving cost performance [7]. The use of phytoremediation to extract toxic elements is less expensive and simpler than the traditional extraction methods. Phytoremediation can also be used for the centralized collection of combustion and power generation [8]. Mulberry is a perennial woody plant with well-developed roots, a fast growth rate, large biomass, strong adaptability, and easy establishment and management. It plays an important role in the remediation of toxic elements in soil, particularly in mine soil [9].
As is harmful to plants. Usually, the first exposed plant tissue is the root, which inhibits the extension and proliferation of roots. After being transferred to the aboveground part, As can seriously inhibit plant growth by slowing or preventing expansion and biomass accumulation and damage plant reproductive capacity by losing fertility, yield, and fruit yield [10]. Root exudates are a wide variety of compounds secreted or released from different parts of the root system into the growth medium during plant growth. Root exudates are abundant and have significant effects. It is a key factor in maintaining the vitality of the rhizosphere microecosystem and an important part of the rhizosphere material cycle. Root exudates significantly alter the physical, chemical, and biological properties of the root-soil interface, thus playing a crucial role in the bioavailability of various nutrients in the soil [11–13]. Environmental stress and plant species have important effects on root exudates. Studies have shown that As can stimulate the secretion of organic acids in As hyperaccumulator Pteris vittata [14]. In addition, it is crucial to understand how plants absorb and metabolize As, to evaluate the phytoremediation of different varieties and screen out varieties with higher enrichment [15].
In this study, three different varieties of mulberry were planted in soils with excessive arsenic (As) content in the Shilu mine dump in Hainan Province. The reduction in As content in the soil and the accumulation of As in different mulberry varieties were analyzed and compared. Metabolomics was used to examine the variations in root exudates to understand the correlation between the differences in As accumulation and transfer in the mine soil of the various mulberry varieties and the root exudates of the mulberry. This study aimed to identify the types of root exudates that can enhance the ability of the root system to adsorb more As and the variances in the types and quantities of root exudates of mulberry that can thrive well in the soil of a waste dump. To better remediate As pollution in mine soil, enhance the healthy development of soil, and ensure human safety, it is essential to modify the type, composition, and quantity of mulberry root exudate.
Materials and Methods
Soil Sample Collection
Soil sampling points were arranged based on the principle of one point per 30 acres at the dumping site of the Shilu Iron Mine in Changjiang, Hainan Province. Three soil sampling points were arranged, and ten samples were collected and mixed at each point. The sampling depth was 0–20 cm of soil excavated, and small rocks and other non-soil components were removed. According to the quartering method, 1 kg of mixed soil was collected from each point to determine the pH and element content of As, Cd, Pb, Ni, and Cr. The remaining soil was filled in the flowerpots to plant mulberry seedlings for the As accumulation experiment and root exudate analysis.
Pot Experiments
The three mulberry varieties selected were Guisangyou 12 (hereafter referred to as G12), Guisangyou 62 (hereafter referred to as G62), and Yuesang 120 (hereafter referred to as Y120), all of which were one-year-old seedlings planted at the same depth. Tropical and subtropical cultivars have high yields and strong resistance. In the experiment, 30 plants of each of the three varieties with similar growth were randomly selected and uniformly trimmed to a height of 15 cm. Individual plants were planted in a flowerpot (33 cm diameter × 22 cm height) containing 10 kg of soil from a waste dump. The spacing between each flowerpot was approximately 10 cm, and the plants were watered at eight o’clock every morning to maintain the relative humidity of the soil at 60–70%. After 60 days, the plants were measured and the root exudates were collected. Consequently, the soil and mulberry trees were sampled separately to determine the element content of As. At the same time, three mulberry varieties were planted in normal soil to compare their growth and developmental differences with those of mulberry varieties planted in the soil of a waste dump.
Measurement and Analysis of Plant Height and Root Length
After 60 days of growth, nine mulberry trees were selected from each of the three mulberry varieties to measure plant height, root length, leaf number, and dry weight.
Collection of Mulberry Root Exudates
After 60 days of growth, nine strains of each mulberry variety were selected and divided into three groups, three strains, and one group. After cleaning the roots with ultrapure water, a single plant was placed in a plastic bottle containing 200 mL of ultrapure water (500 mL), wrapped with tin foil to prevent photodegradation, and placed in situ to collect root exudates [16]. After 20 hours, the plants were removed from the bottle, and the root exudates were mixed into a group of three strains before being transferred into the cryopreservation tube. After cryopreservation in liquid nitrogen, the samples were brought back to the laboratory for determination and analysis of root exudates.
Soil and Mulberry Sample Collection
Nine strains from three mulberry varieties were randomly selected and divided into three groups, three strains and one group. Each group of soil and mulberry samples was separated. Then, (1) 1000 g of each soil group was evenly mixed, ground, and passed through a 100-mesh sieve to determine the element content of As. (2) Washing the soil on the plant with ultrapure water, separating the roots, stems, and leaves, drying them in the oven at 70°C, measuring the dry weight of the plant, grinding them, passing through a 100-mesh sieve, and determining the element content of As.
Detection and Analysis of Root Exudates
The freeze-dried powdered root exudate solution was removed, 100 μg of the sample was weighed, and 1000 μL of the extract (methanol: acetonitrile: water = 2:2:1, v/v) was added and mixed by shaking. Ultrasonic treatment was performed in an ice-water bath for 10 min, followed by rapid freezing in liquid nitrogen for 1 min. This process was repeated three times. The sample was stored at -20°C for 1 hour and centrifuged at 13, 000 rpm for 15 min at 4°C. The supernatant was collected and dried using a nitrogen-blowing instrument. Approximately 100 μL acetonitrile: water = 1:1 (v/v) was added to re-dissolve the solution. The mixture was shaken for 30s and ultrasonicated in an ice water bath for 10 min. The mixture was centrifuged at 13, 000 rpm for 15 min at 4°C. The supernatant was diluted with liquid chromatography-mass spectrometry (LC-MS) grade water containing 53% methanol. The diluted supernatant was centrifuged and injected into a Vanquish UHPLC system (Thermo Fisher, Germany), and the metabolites were analyzed using an Orbitrap Q Exactive TM HF mass spectrometer (Thermo Fisher, Germany).
Determination of As in Soil and Plants
Accurately weighed 0.20 g of soil samples, added 5ml of hydrochloric acid after a little water infiltration, heated and evaporated to 2–3 ml at low temperature, added concentrated HNO3 (5 ml), HF (2 ml), and HClO4 (2 ml) in turn, heated to fully decompose organic carbides and evaporated to a viscous liquid, repeated digestion, cooling, 1 % HNO3 rinsed and filtered in a 25 ml colorimetric tube, and diluted to 25 ml [17].
Weigh 0.50 g of plant samples, add 5 ml of concentrated HNO3, and soak overnight. Then add 10 ml of concentrated HNO3, 5 ml of HClO4 heated to evaporate until transparent, continue to evaporate to the solution to produce thick white smoke, cool, 1% HNO3 rinsed and filtered in 25 ml colorimetric tube, constant volume to 25 ml [17].
Total As concentrations were determined by an atomic fluorescence spectrometer (AFS-8220, Beijing Jitian Instruments Co., Ltd., China) [17]. Quality assurance and quality control were performed for each batch of samples. The standard reference materials (GBW07407 for soil, GBW10020 for plant) from the National Standard Substances Center of China were observed throughout the digestion and subsequent analysis. The total As recovery was 94.6–101.5% for the soil samples and 95.6–104.7% for the plant samples.
Data Analysis
Pollution index (Pi): the measured content of pollution elements in soil/the evaluation standard of soil pollution elements [18].
Pi ≤ 1 indicates no pollution, 1.0 < Pi ≤ 2.0 indicates mild pollution, 2.0 < Pi ≤ 3.0 indicates moderate pollution, and Pi > 3.0 indicates severe pollution.
Transfer coefficient (TF): the content of elements in the aboveground part of the plant/the content of elements in the underground part of the plant.
Enrichment factor (BCF): the content of elements in plants/the content of corresponding elements in soil.
Microsoft Excel 2016 was used to calculate and analyze the plant height, root length, and other parameters of the different mulberry varieties. It was also used to determine the element pollution index of the rhizosphere soil, the enrichment coefficient of elements in different mulberry varieties, and the migration coefficient of the five elements in mulberry. IBM SPSS Statistics 25 was used to analyze significant differences using a one-way analysis of variance (ANOVA) followed by Duncan’s multiple-range test.
For metabolomic analysis of root exudates, principal component analysis (PCA) and partial least squares discriminant analysis (PLS-DA) was performed using the R package ropls version 1.6.2. The robustness of the model was assessed based on the model evaluation parameters (R2 and Q2) to avoid overfitting. A projection value (VIP) > 1.0, p = 2, or < 0.5 was of great significance for the selection of differential metabolites. The robustness of the PLS-DA model was verified using 200 response permutation tests (RPTs). Metabolism pathway analysis was performed using the Kyoto Encyclopedia of Genes and Genomes (KEGG, https://www.genome) in the pathway analysis module of MetaboAnalyst 5.0 (https://www. metaboanalyst.ca/home.xhtml). (jp/kegg/pathway.html) and (Human Metabolome Database (HMDB, https://hmdb. ca/metabolites). Metabolic pathways with a path influence value (PIV) > 0 and − log10 (P) > 1 were considered as potential interfering pathways [19]. Differentially expressed metabolites were screened by combining the fold changes and VIP values. Metabolites with a fold change ≥ 2, ≤ 0.5, and ≥ 1 were selected as significant differential metabolites.
Results and Discussion
Effects of Soil from Waste Dumps on the Growth of Different Mulberry Varieties
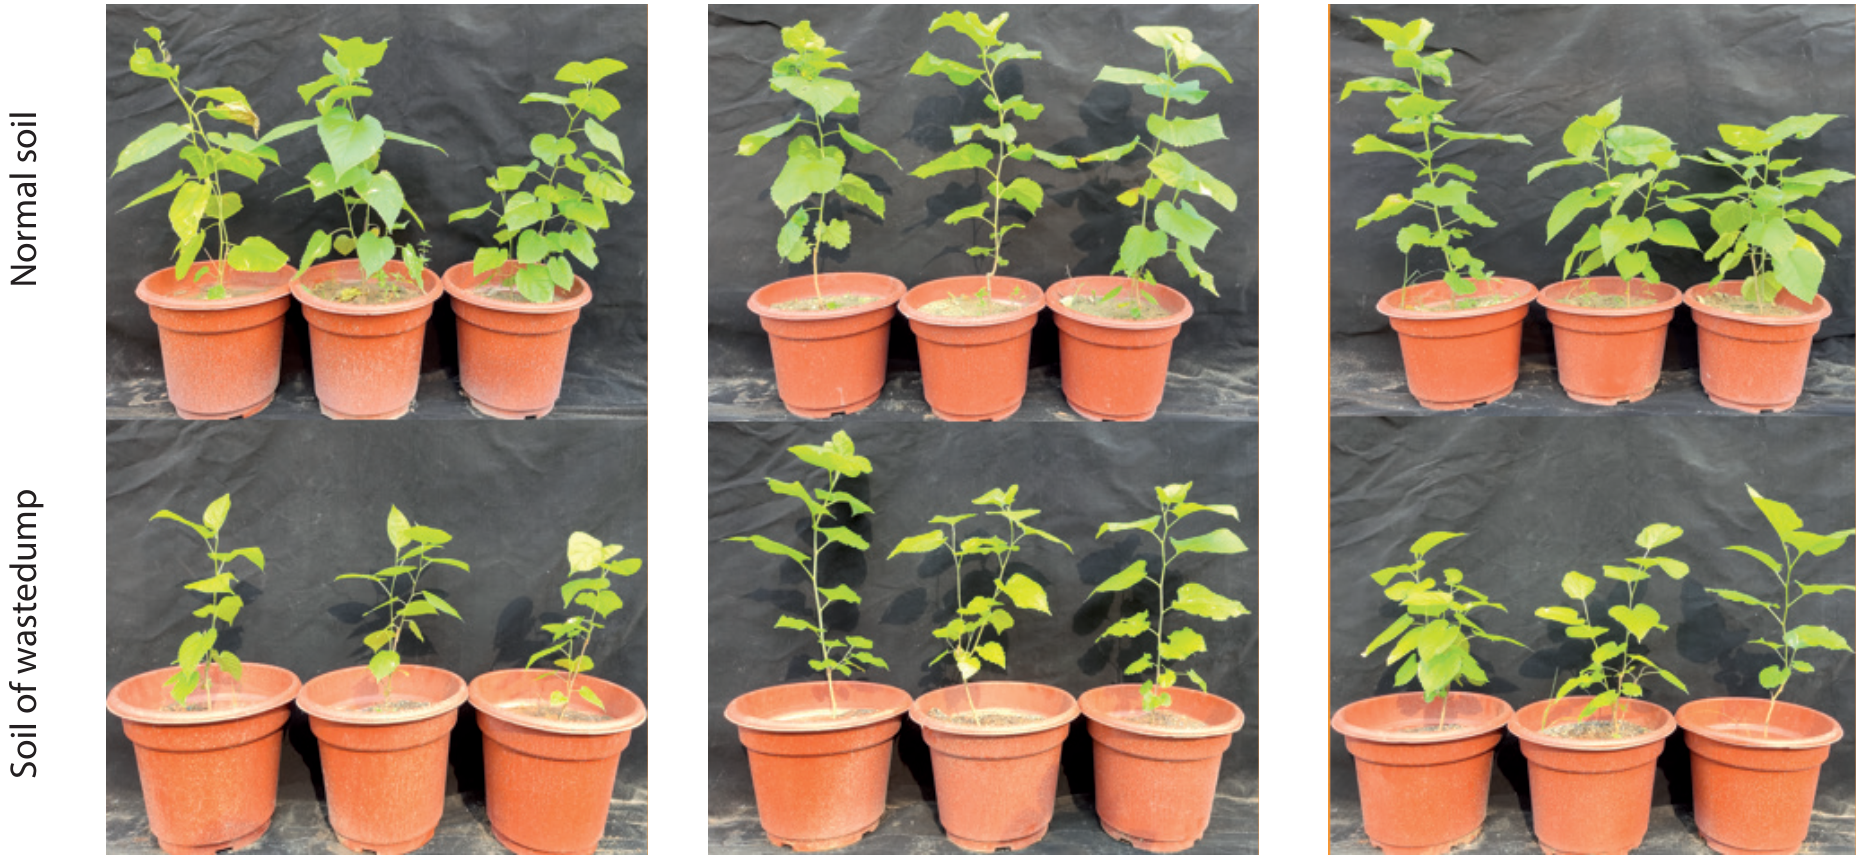
After 60 days of planting in As-excess soil from waste dumps in the Shilu mine, the height of the aboveground parts of the three mulberry varieties (G12, Y120, and G62) decreased by 21.66 cm (41.14%), 14.33 cm (33.53%), and 19.66 cm (22.63%), respectively, compared with that in the normal soil. G12 decreased the most, and G62 decreased the least. After planting in soil from a waste dump, the number of branches and leaves of G62 increased, while the number of leaves of G12 decreased significantly. In addition, the drying weight of the three mulberry varieties was significantly lower than that of normal soil planting (P < 0.01). G12, G62, and Y120 decreased by 91.89 g (54.68%), 79.13 g (41.44%), and 96.16 g (51.93%), respectively, among which G62 decreased the least (Fig. 1 and Fig. 2).
Analysis of Element Content in Soil before and after Planting Different Mulberry Varieties
The nutrient parameters of soil from a waste dump and normal soil are presented in Table 1, which indicates that the overall soil nutrient content was low. The pollution index of As was 3.63, indicating severe pollution, whereas the other elements, Cd, Pb, Ni, and Cr, were all pollution-free (Table = 2). Sixty days after planting the three mulberry varieties, the pH values of the rhizosphere soil decreased. Specifically, G12, G62, and Y120 exhibited pH values of 7.9, 7.6, and 8.1, respectively. The content of As in the rhizosphere soil of G12, G62, and Y120 decreased from 91.30 mg·kg-1 to 83.14 mg·kg-1 (a decrease of 8.94%), 85.46 mg·kg-1 (a decrease of 6.40%), and 87.54 mg·kg-1 (a decrease of 4.12%). Although the pollution level in the rhizosphere soil remained high, the pollution index decreased (Table 3).
Accumulation and Transfer Ability of Different Mulberry Varieties for As
The mass fraction of As in the rhizosphere soil of the three mulberry varieties remained heavily polluted 60 days after planting in the As-exceeding soil from waste dumps. However, the pollution index decreased. Compared with the other two mulberry varieties, the transport and accumulation of As in the leaves of G62 were significantly higher than those of G12 and Y120. This resulted in the highest transfer ability of As in the aboveground part of G62, which was significantly higher than that of the other two varieties. However, the enrichment coefficients were lower (Table 4). The accumulation of As in the three mulberry varieties followed the order of G62 (9.27 ± 1.57 mg·kg-1) > Y120 (8.72 ± 1.50 mg·kg-1) > G12 (7.97 ± 1.46 mg·kg-1). Additionally, the transport capacity of As was observed to be in the order root > leaf > stem. The amount of As transported by the aboveground plant parts was nearly equal to that of the roots. The percentage of As accumulated in the roots relative to that in the total plant was as follows: 52.02% (Y120) > 51.78% (G12) > 47.99% (G62). The percentage of As accumulated in the roots relative to that in the total plant was as follows: 37.22% (G62) > 32.98% (G12) > 30.01% (Y120). G62 leaves accumulated the highest amount of As.
Effects of Soil from Waste Dumps on Root Exudates of Different Mulberry Varieties
Analysis of Metabolic Pathway Differences in the Root Exudates
The primary chemical grouping of 296 identified metabolites from mulberry varieties planted in soil from waste dumps compared with normal soils was analyzed through over-representation analysis using metabolite set enrichment analysis (MSEA) (Fig. 3, Tables 5 and 6). Three mulberry varieties were planted in normal soil and soil from waste dumps for 60 days. A total of 296 root exudates were detected, including 88 organic acids and derivatives, 59 organic oxygen compounds, 40 nucleotides and analogs, and 30 lipids and lipid-like molecules. Organoheterocyclic compounds 23, benzenoids 20, phenylpropanoids and polyketides 12, organic nitrogen compounds 10, lignans, neolignans and related compounds 1, alkaloids and derivatives 1, and others 12. Phosphoserine and uridine diphosphate-N-acetylglucosamine were newly detected in soil from waste dumps compared with normal soil. Nine compounds were not detected (2‘-deoxycytidine 5‘-monophosphate (dCMP), dimethylallyl diphosphate, glutathione reduced, S-adenosylhomocysteine, inosine triphosphate (ITP), N2, N2-dimethylguanosine, norleucine, protirelin, and vitamin B2).
Fig. 2.
Plant height, root length, leaf number, and dry weight of different mulberry varieties planted in soil from a waste dump for 60 days.
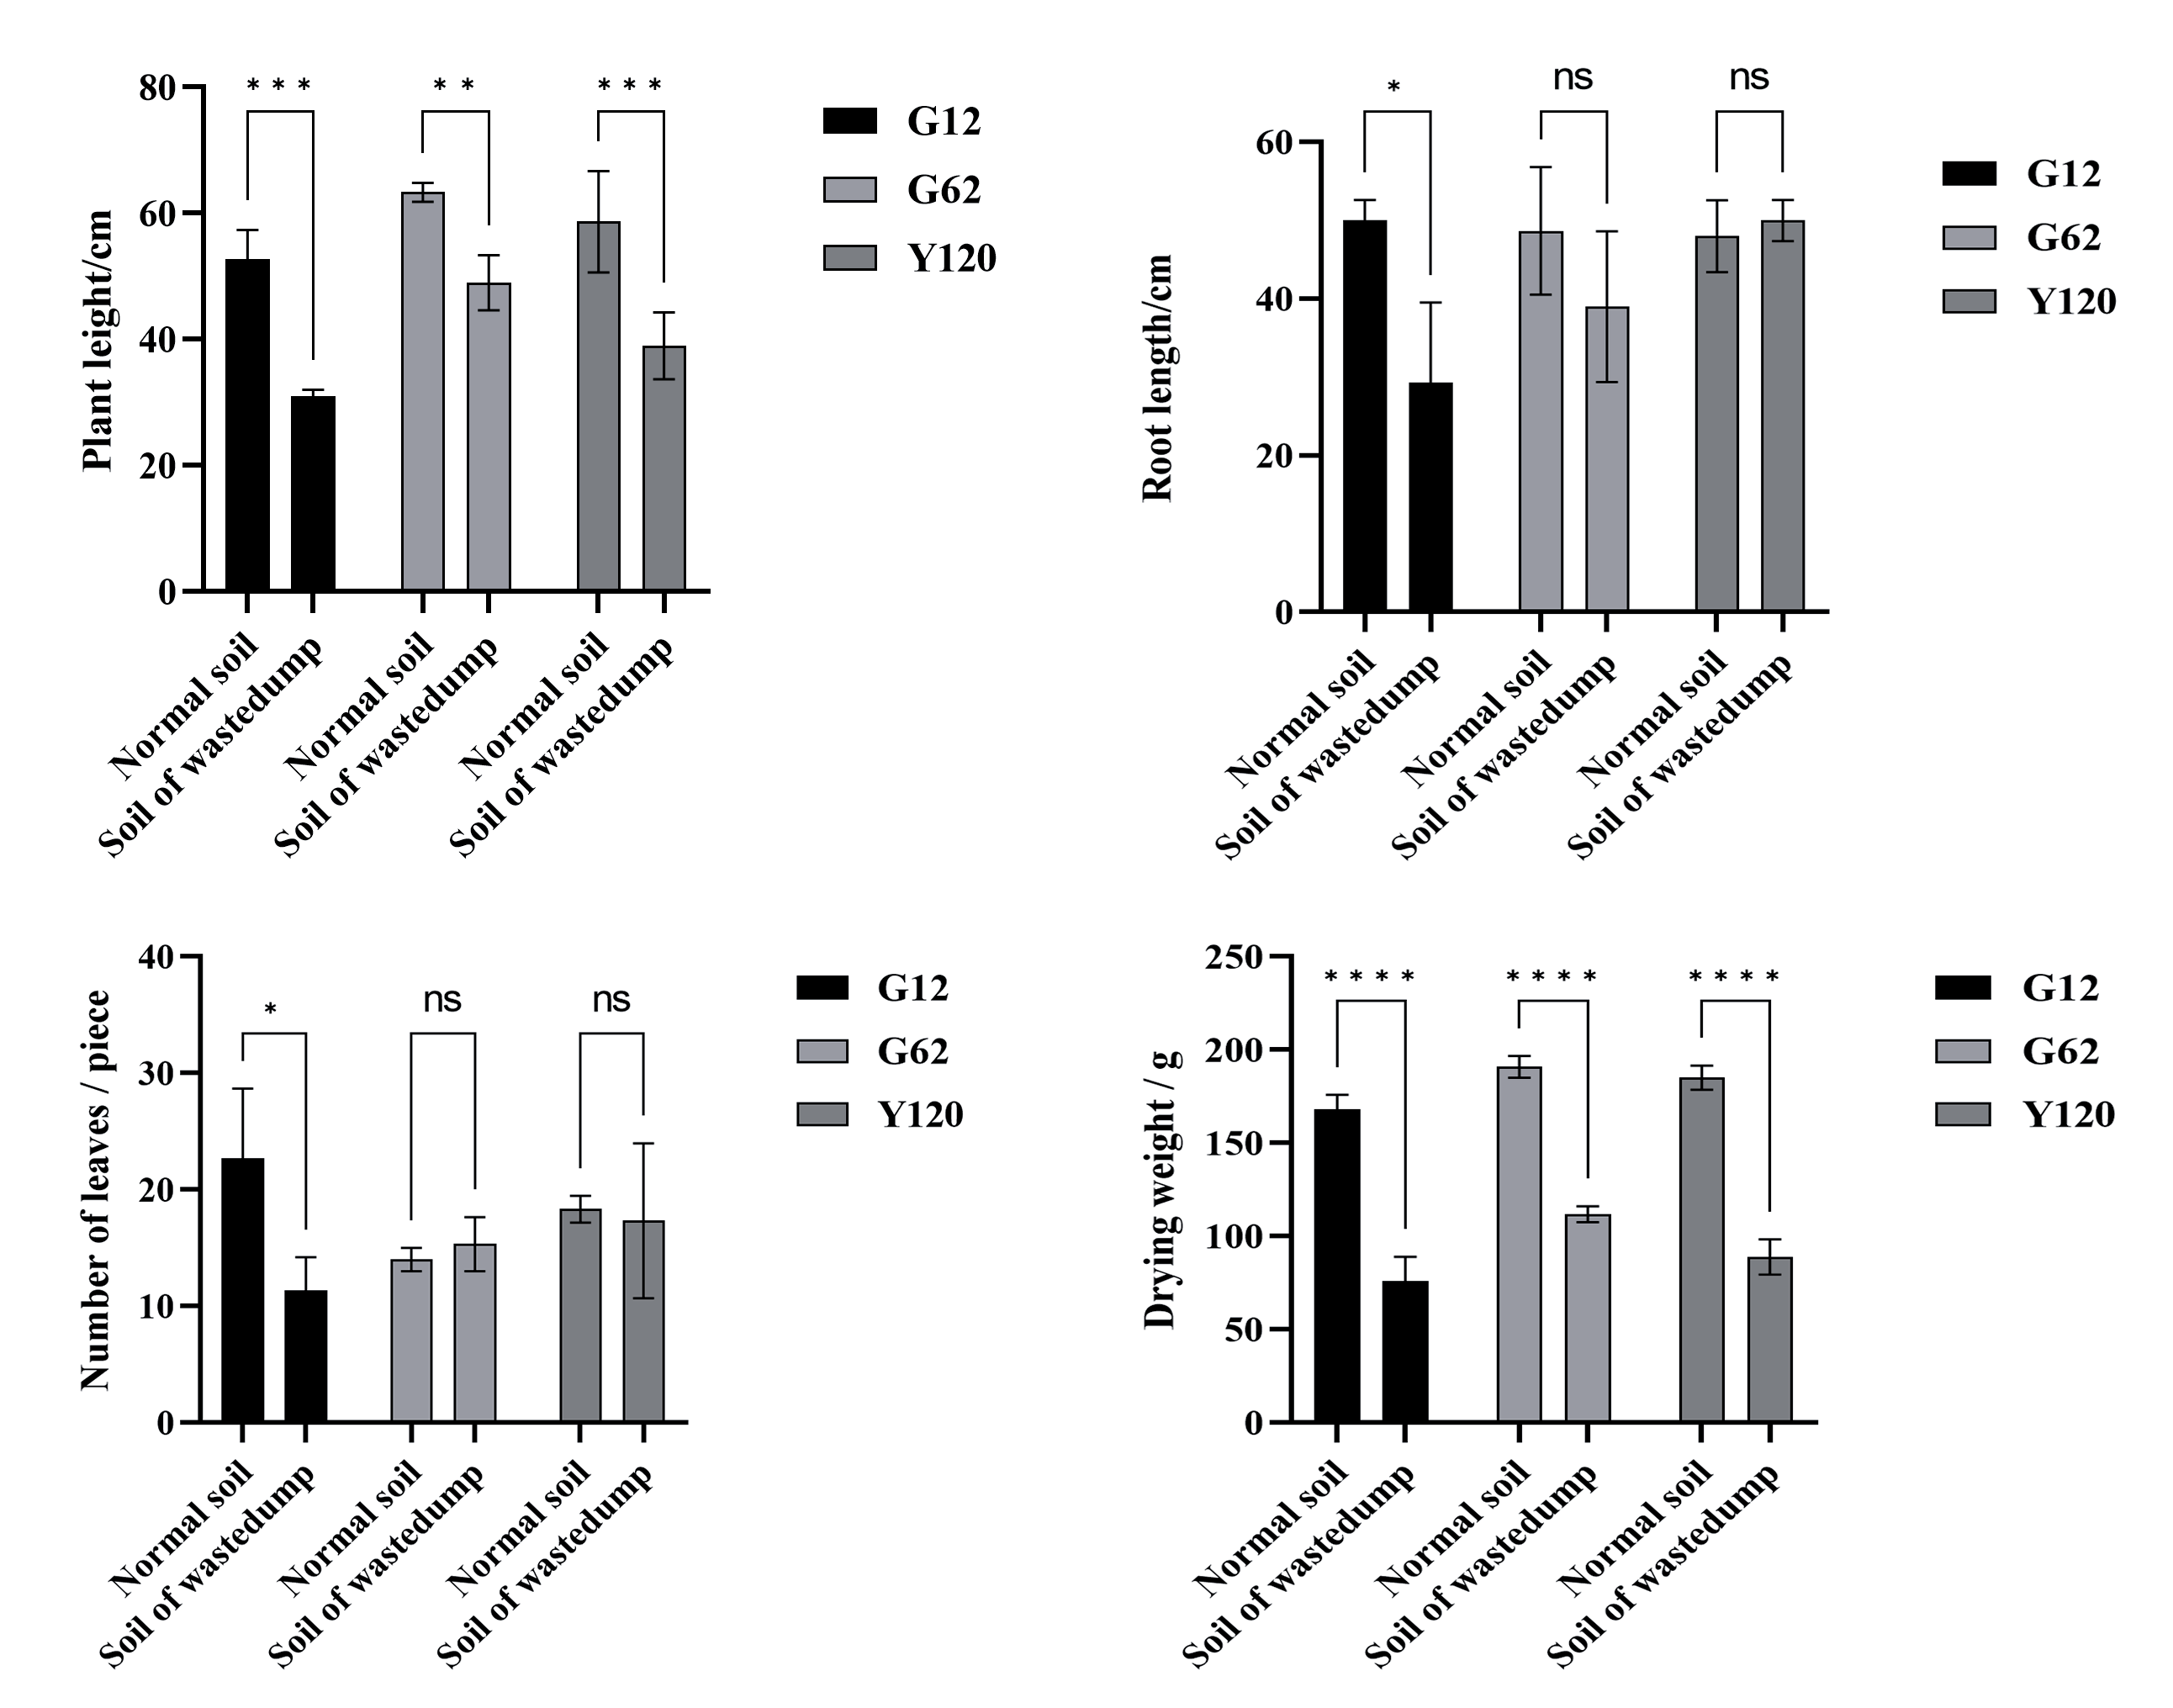
Table 1.
Nutrient parameters of soil from waste dumps.
Table 2.
Distribution of toxic element species in soil from waste dumps.
Table 3.
Changes in As content and pollution in soil before and after planting different mulberry varieties.
Table 4.
Mass fractions of As in various parts of different mulberry varieties and rhizosphere soils.
Compared with normal soil cultivation, there were 16 metabolic pathways involved in the first 25 important metabolic pathways in the three varieties. Among them, the effects on galactose metabolism varied significantly among the three varieties. The effects were more pronounced in G62 and Y120, which exhibited the best growth and the highest As accumulation. In contrast, the effects were relatively small in G12, which showed the poorest growth and limited the aboveground As transfer. The pentose phosphate pathway, starch and sucrose metabolism, and citrate cycle (TCA cycle) exhibited significant changes in G62. The main chemical groups with a higher p-value were amino acids and peptides, fatty acids and conjugates, monosaccharides, pyrimidines, and TCA acids in the three mulberry varieties grown in soil from waste dumps compared with normal soils (Fig. 3B, D, F, Table 5).
As all 296 metabolites were identified, over-representation analysis of MSEA indicated significant chemical groups within the chemical structure metabolite sets (top 25) with enrichment ratios (Fig. 3B, D, F, Table 6).
Compared with normal soil cultivation, the amount of root exudates of the three mulberry varieties changed significantly 60 days after planting in soil from waste dumps (Fig. 4 A, B, C). Among them, 19 metabolites in G12 increased significantly and 42 metabolites decreased significantly (Fig. 4 D, G). In G62, 52 metabolites increased significantly and 42 metabolites decreased significantly (Fig. 4 E, G). Additionally, 48 metabolites in Y120 increased significantly, whereas 37 metabolites decreased significantly (Fig. 4 F, G).
Effect on Organic Acid Secretion
Compared with normal soil planting, significant differences were observed in the content of 26 organic acids secreted by the roots of the three mulberry varieties 60 days after planting in soil from waste dumps. Specifically, 16 organic acids were found in G62, 13 in G12, and 3 in Y120. (Fig. 5). Citrate, 2-Aminooctanoic acid, and p-Coumaric acid were significantly increased in the three mulberry varieties. Ten species (Alpha-Ketoglutarate, Pyruvate, Succinate, D-(-)-Quinic acid, Fumatrate, Quinic Acid, Isocitrate, Taurine, Glucose 1-phosphate and Aniline-2- sulfonate) were significantly increased in G12 and G62. In particular, Alpha-Ketoglutarate, Pyruvate, Succinate, Citrate, and D-(-)-Quinic acid increased by 40.82, 16.85, 7.43, 6.36, and 4.51 times in G62 to 40.82, 16.85, 7.43, 6.36, and 4.51 times in normal soil cultivation, and increased by 3.81, 4.40, and 9.10, 6.44, and 8.63 times in G12. Four compounds (L-Malate acid, trans-Aconitic acid, Phosphoenolpyruvate, and Madasiatic acid) were only significantly increased in G62, but decreased in G12 and Y120. These results indicate that the increase of organic acids, especially Alpha-Ketoglutarate and Pyruvate, may help G62 to better adapt to soil from waste dumps and promote its growth, which may also be an adaptation pathway and strategy of mulberry to arsenic stress.
Fig. 3.
Root exudate difference analysis of the three mulberry varieties planted in soil from waste dumps compared with normal soil based on metabolite set enrichment analysis (MSEA) (A: P-G12 vs N-G12, B: P-G62 vs N-G62, C: P-Y120 vs N-Y120). N-G12, N-G62, and N-Y120 represent three mulberry varieties planted in normal soil, respectively. P-G12, P-G62, and P-Y120 represent three mulberry varieties planted in soil from waste dumps, respectively. P-G12 vs N-G12, P-G62 vs N-G62, and P-Y120 vs N-Y120 represent the root exudates differences of the mulberry variety planted in soil from waste dumps compared with normal soil, respectively.
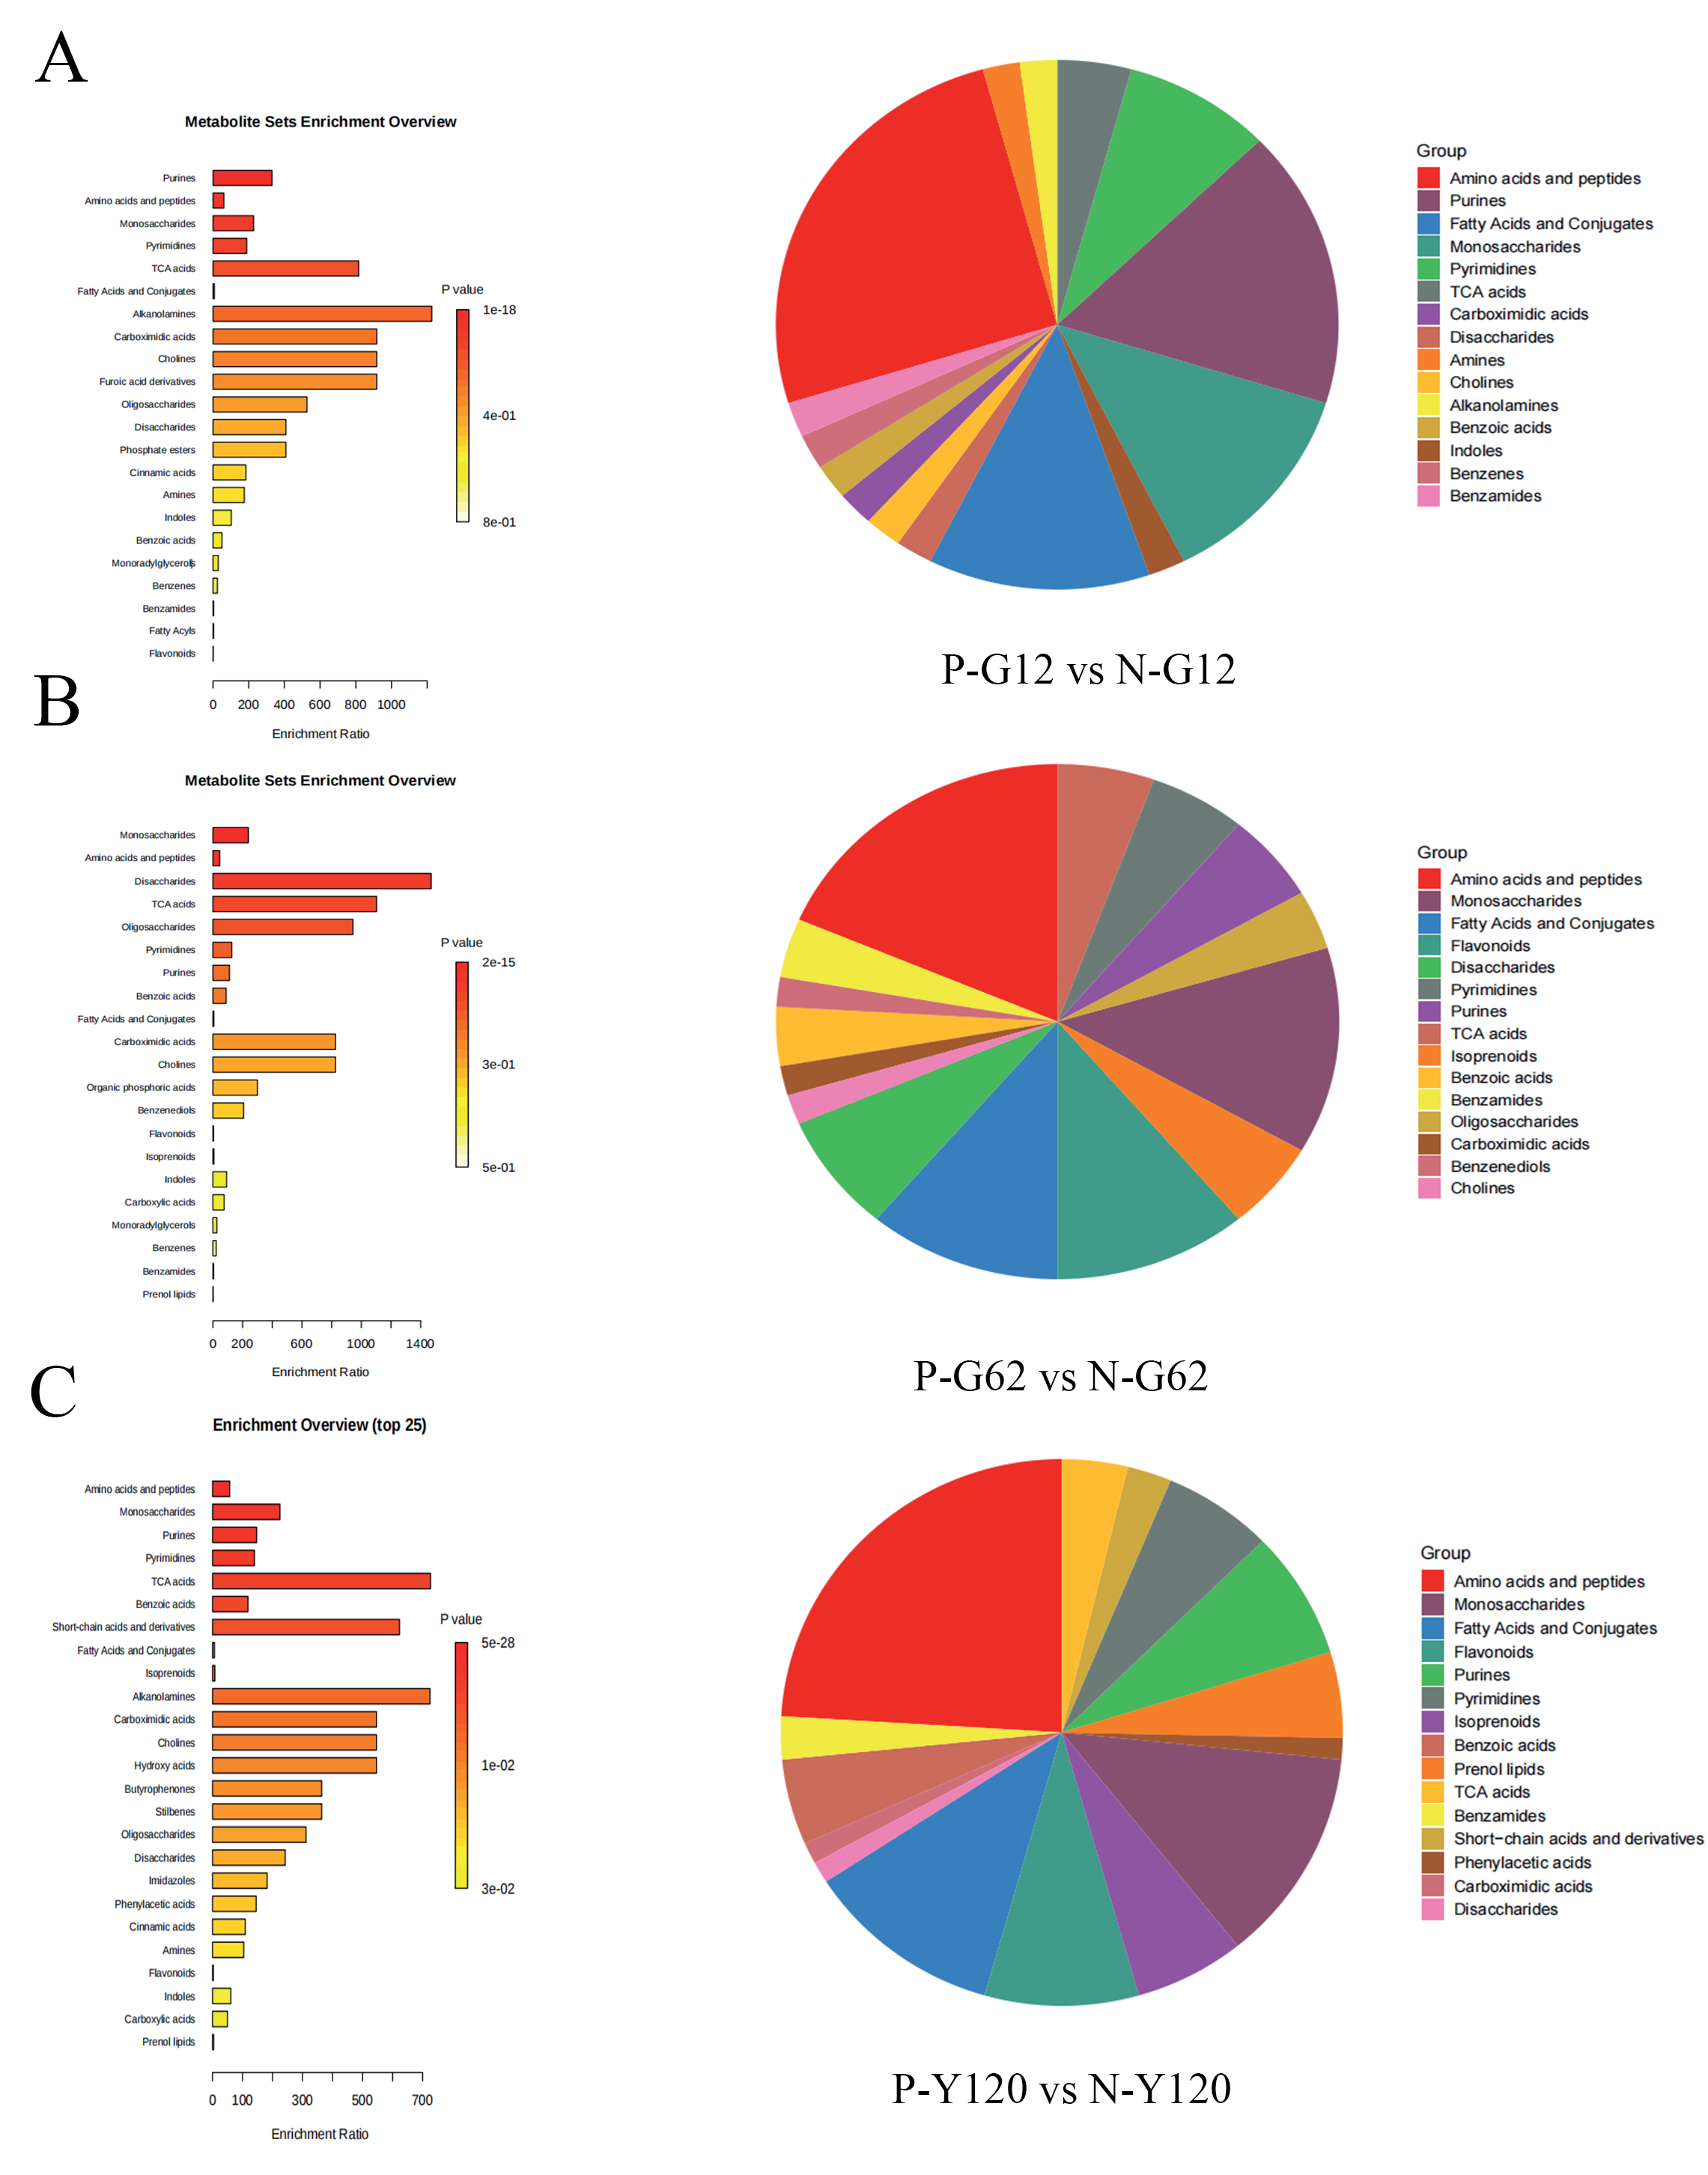
Table 5.
Main chemical groups with a higher p-value in different mulberry varieties planted in soil from waste dumps rather than normal soils.
Seven compounds (2-phosphoglyceric acid, glucuronic acid, 2-hydroxybutyric acid, 2,3-diaminopropionic acid, hydroxypropionic acid, glycerol 3-phosphate, and 6-phosphogluconic acid) were significantly reduced in the three varieties, with 2,3-diaminopropionic acid being the most abundant. It was significantly lower than the normal growth in the three varieties (G62 was reduced to 0.34, G12 was reduced to 0.62, and Y120 was reduced to 0.36), but pipecolic acid was different. It was reduced to 0.34 times the normal roots in accumulated G12 roots, 0.96 times normal roots in G62, and 0.85 times normal roots in Y120 roots. This indicates that 2,3-diaminopropionic acid, and pipecolic acid may not support the adaptation of mulberry plants to As stress.
Effects on Carbohydrate Secretion
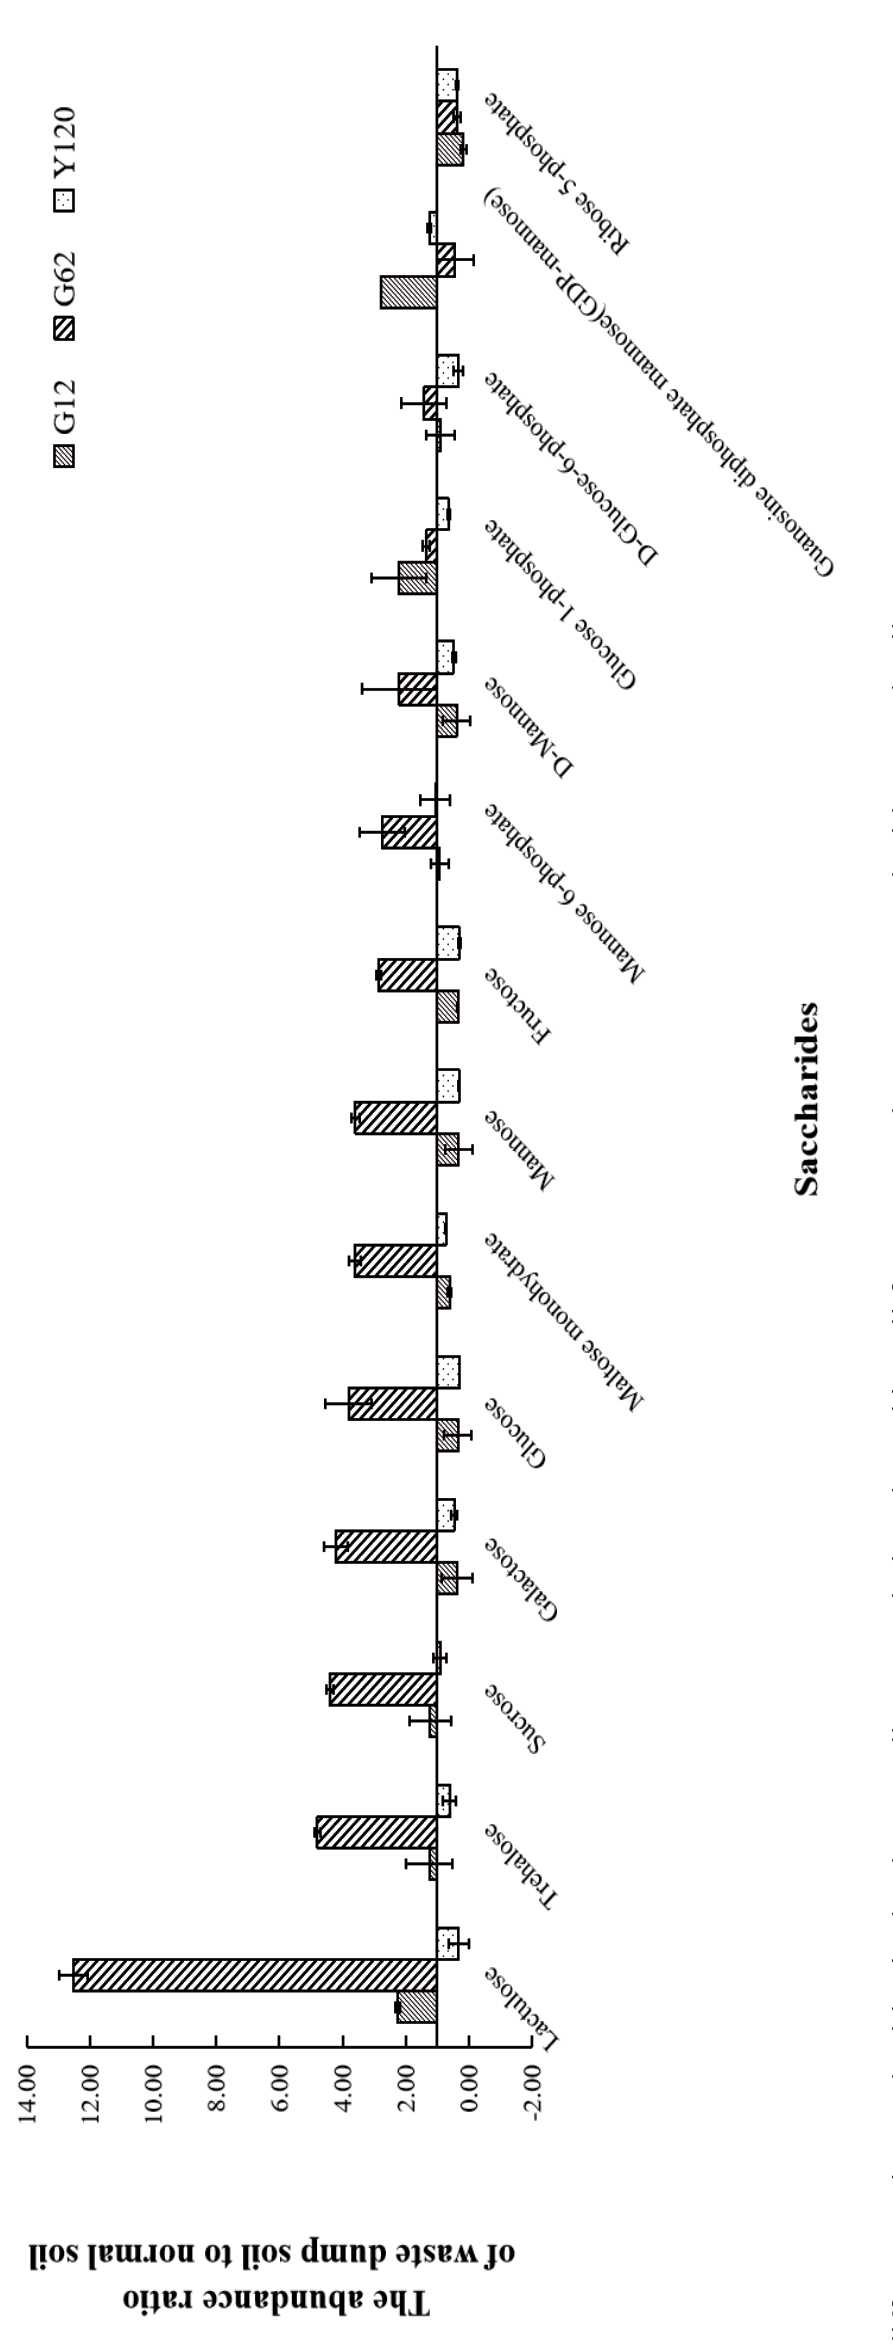
Compared with normal soil, significant differences were observed in the content of 15 main sugars secreted by the roots of three mulberry varieties 60 days after planting in the As-exceeding soil from waste dumps. Specifically, there were 13 sugars in G62, 5 in G12, and 2 in Y120. (Fig. 6). The increase in the 11 sugars in G62 was higher than that in the other two varieties, which may be related to the promotion of branch growth under high As stress. Lactulose, trehalose, sucrose, and glucose 1-phosphate increased significantly in G12 and G62. In particular, lactulose increased by 12.51 times in G62, whereas the other three increased by 4.21–4.80 times in G62. These sugars may help reduce the toxicity of As to mulberry trees and provide nutrients to support their growth, thereby minimizing the impact of soil on their growth.
Table 6.
Quantity of the root exudates annotated to the top 25 metabolic pathways of the three mulberry varieties planted in soil from waste dumps compared with normal soils.
Effect on Amino Acid Secretion
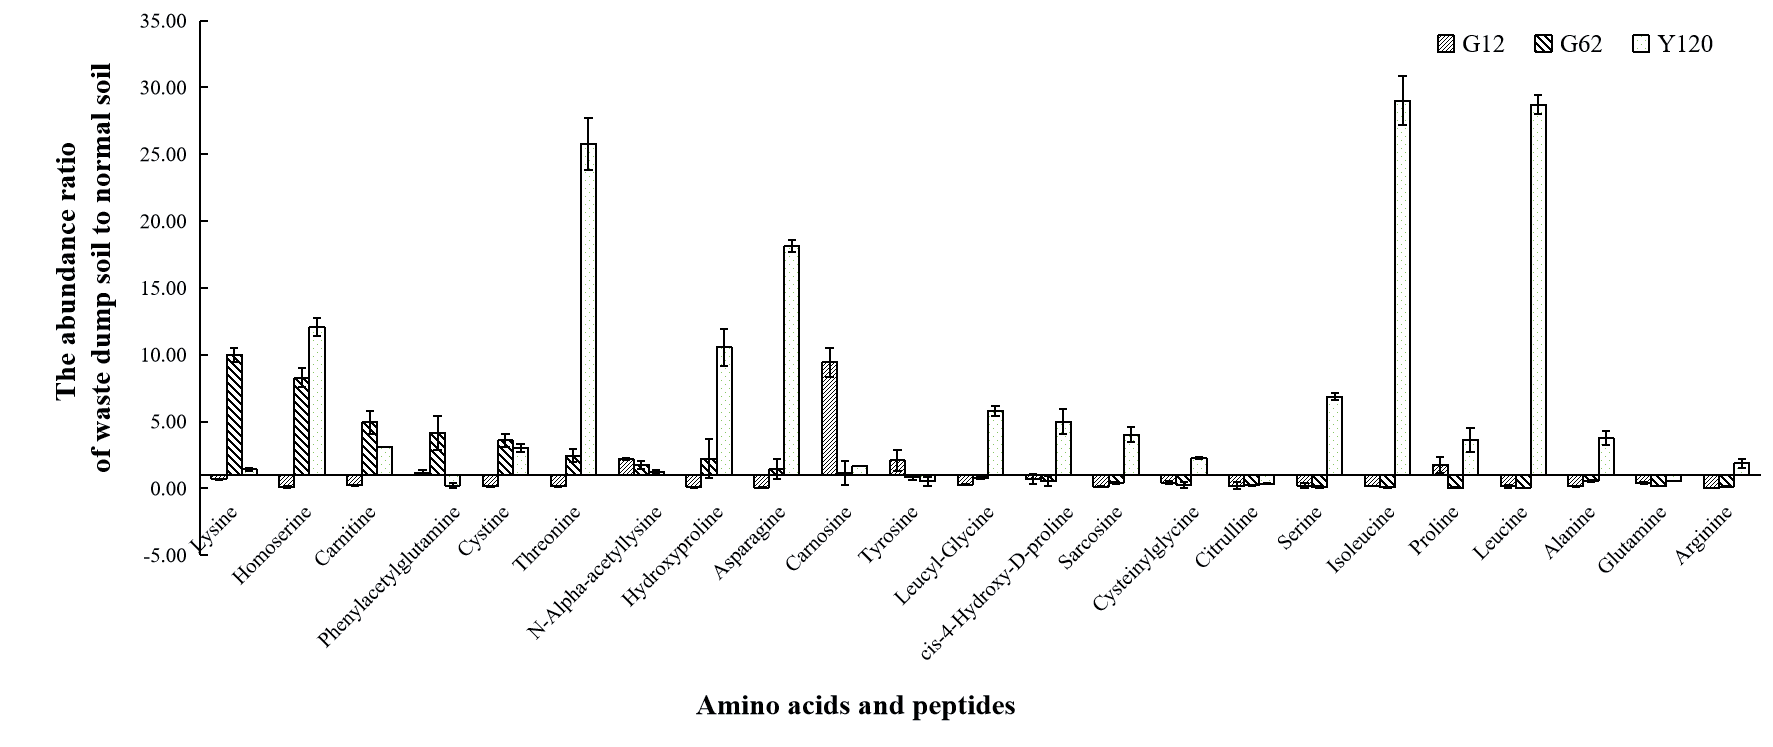
Compared with normal soil planting, the roots of the three mulberry varieties secreted phosphoserine and did not secrete norleucine 60 days after planting in soil from waste dumps. There were 23 amino acids with significant differences in content, including 10 in G62, 4 in G12, and 18 in Y120 (Fig. 7). N-alpha-acetyllysine and carnosine were significantly increased in the three varieties especially, carnosine, which showed the highest increase, reaching 9.43 times the normal root secretion in the least productive G12, indicating that it may help G12 reduce As accumulation, thus playing an important role. Lysine and homoserine increased by 10.00 and 8.26 times in G62 with significant growth and high As accumulation compared with normal soil cultivation and increased by 1.42 and 12.06 times in Y120 with medium growth and enrichment levels, respectively. The increase in four amino acids (lysine, inosine, phenylacetylglutamine, and cystine) in G62 was higher than that in the other two varieties, indicating that these amino acids may be related to reducing the toxicity of more As transferred in G62 and Y120 to reduce the toxicity to mulberry.
Fig. 4.
Compared with normal soil, the root exudates of the three mulberry varieties were different 60 days after planting in soil from waste dumps (A: PCA score plot of P-G12 vs N-G12, B: PCA score plot of P-G62 vs N-G62, C: PCA score plot of P-Y120 vs N-Y120, D: The differential metabolite volcano plot of P-G12 vs N-G12, E: The differential metabolite volcano plot of P-G62 vs N-G62, F: The differential metabolite volcano plot of P-Y120 vs N-Y120, G: Number of up and down-regulated metabolites)
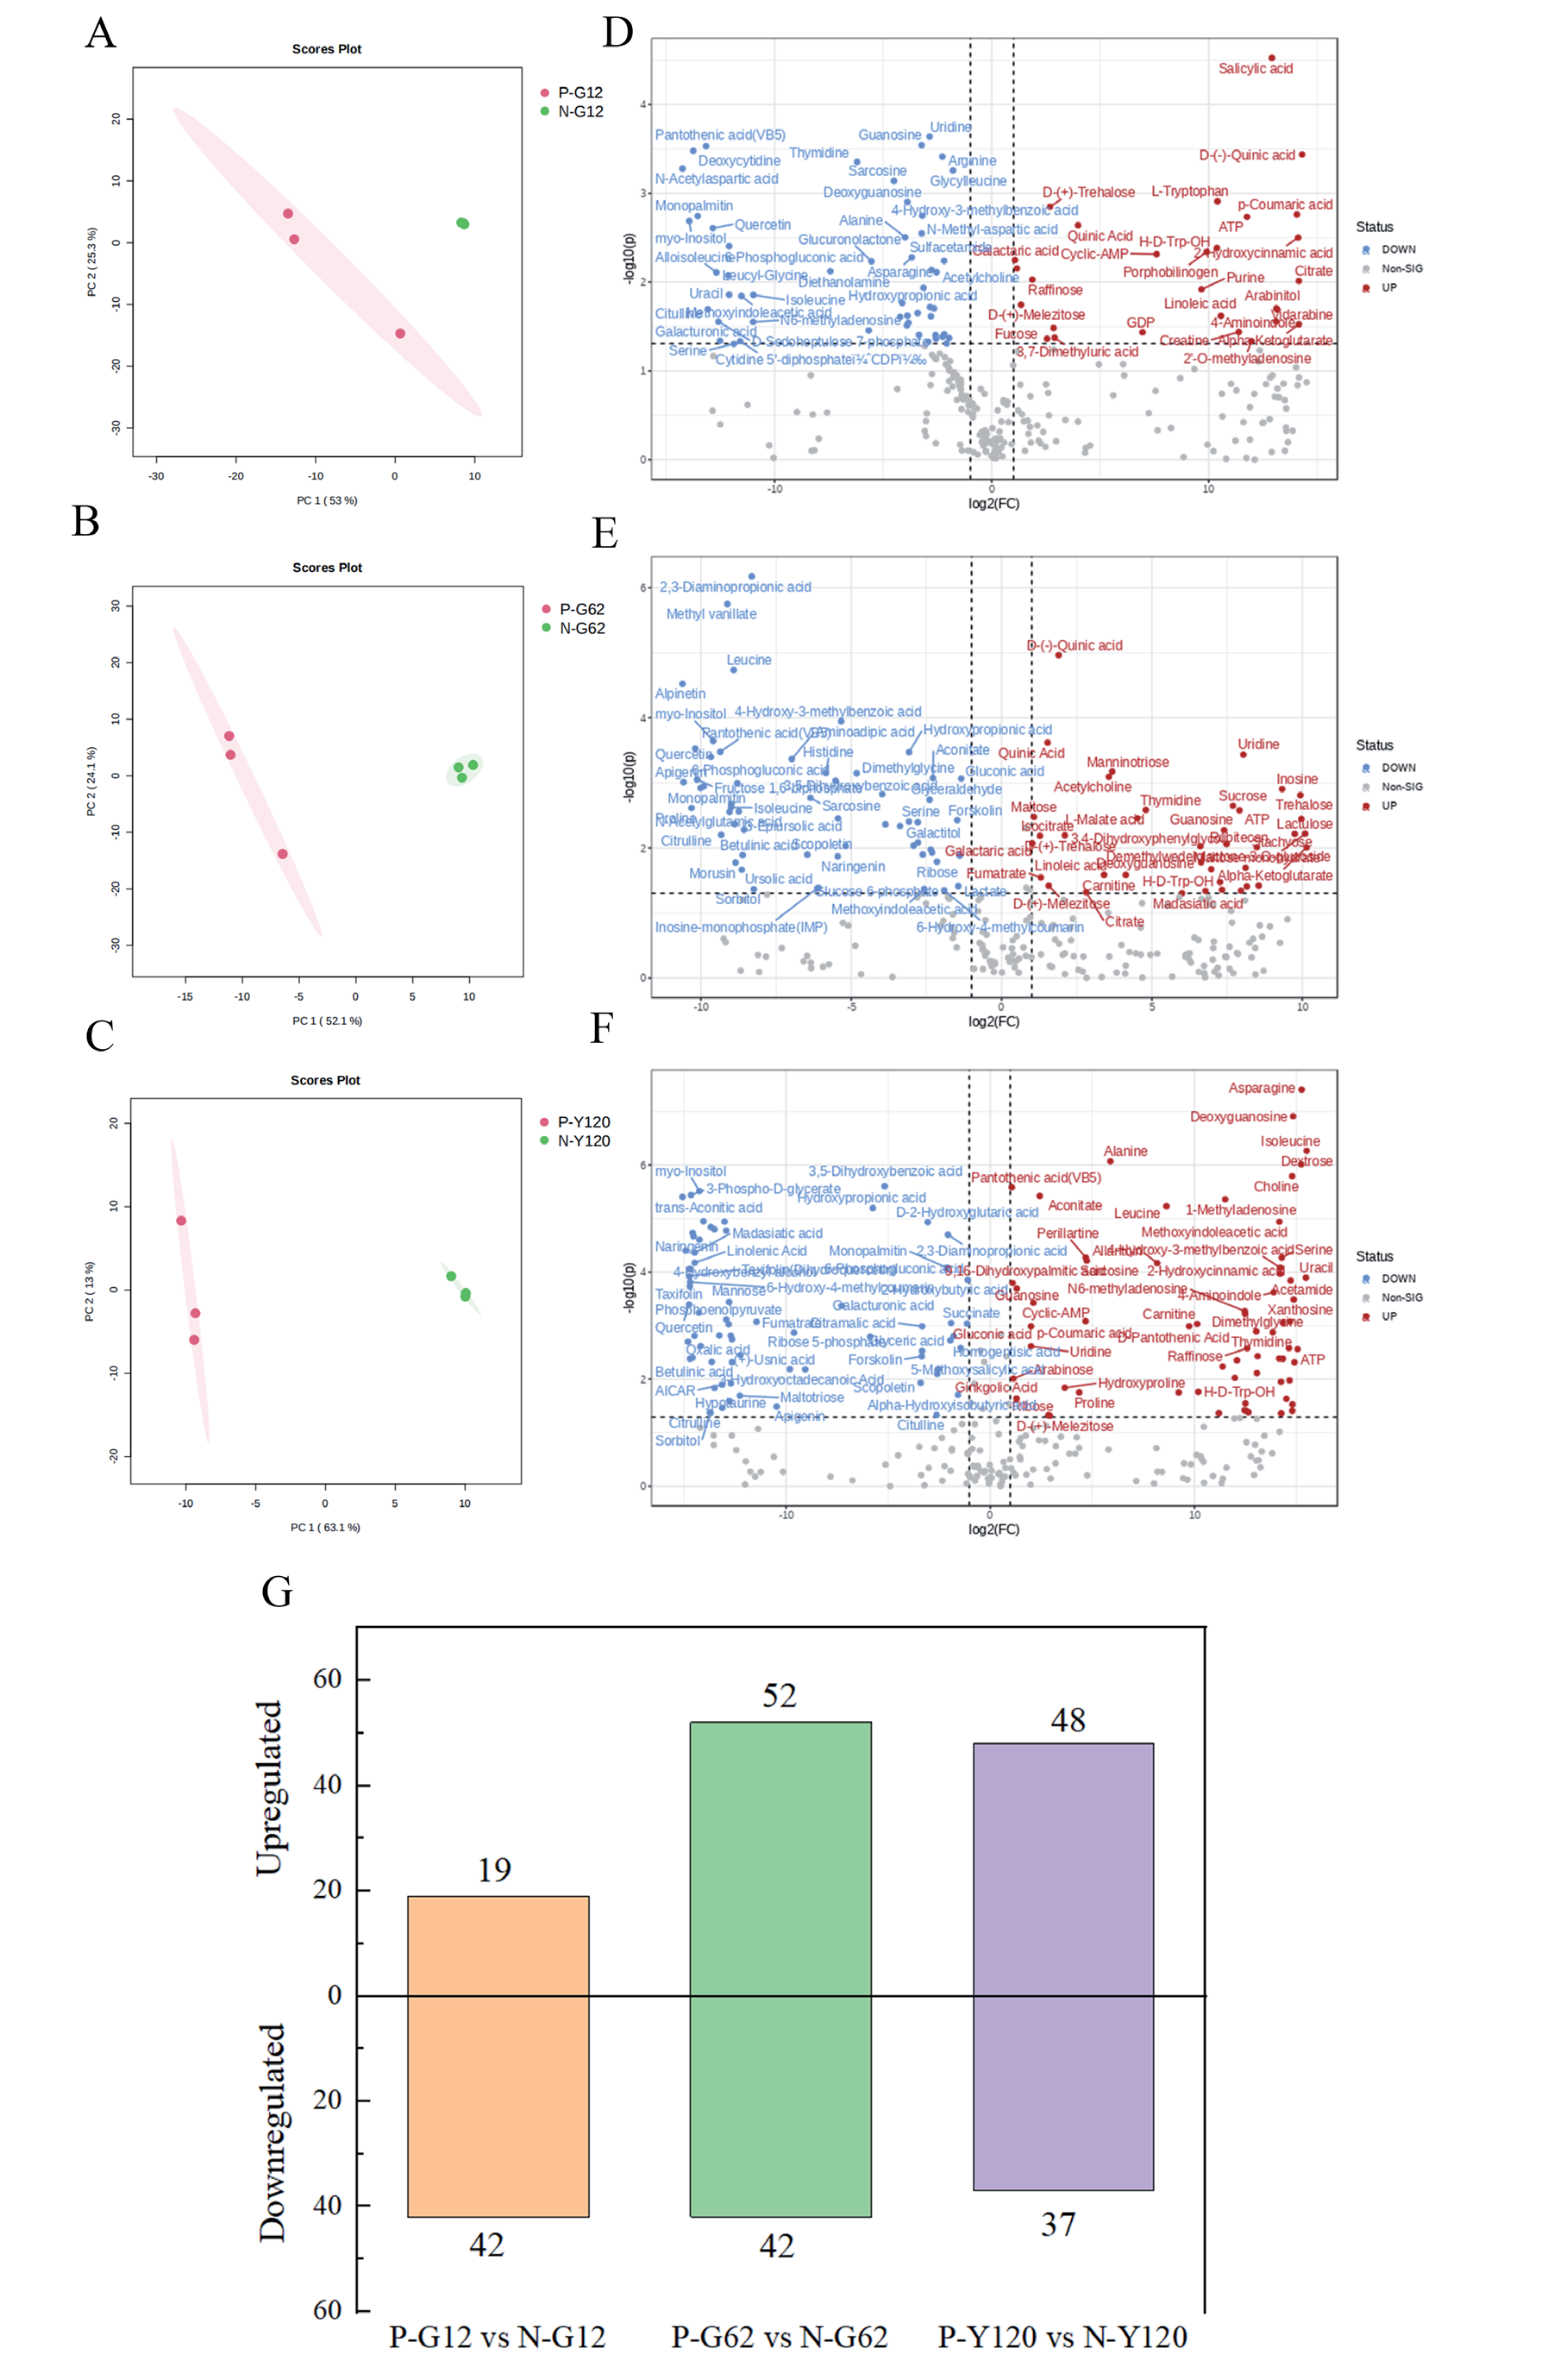
Fig. 5.
Abundance differences in organic acids in the three mulberry varieties planted in soil from waste dumps compared with normal soil.
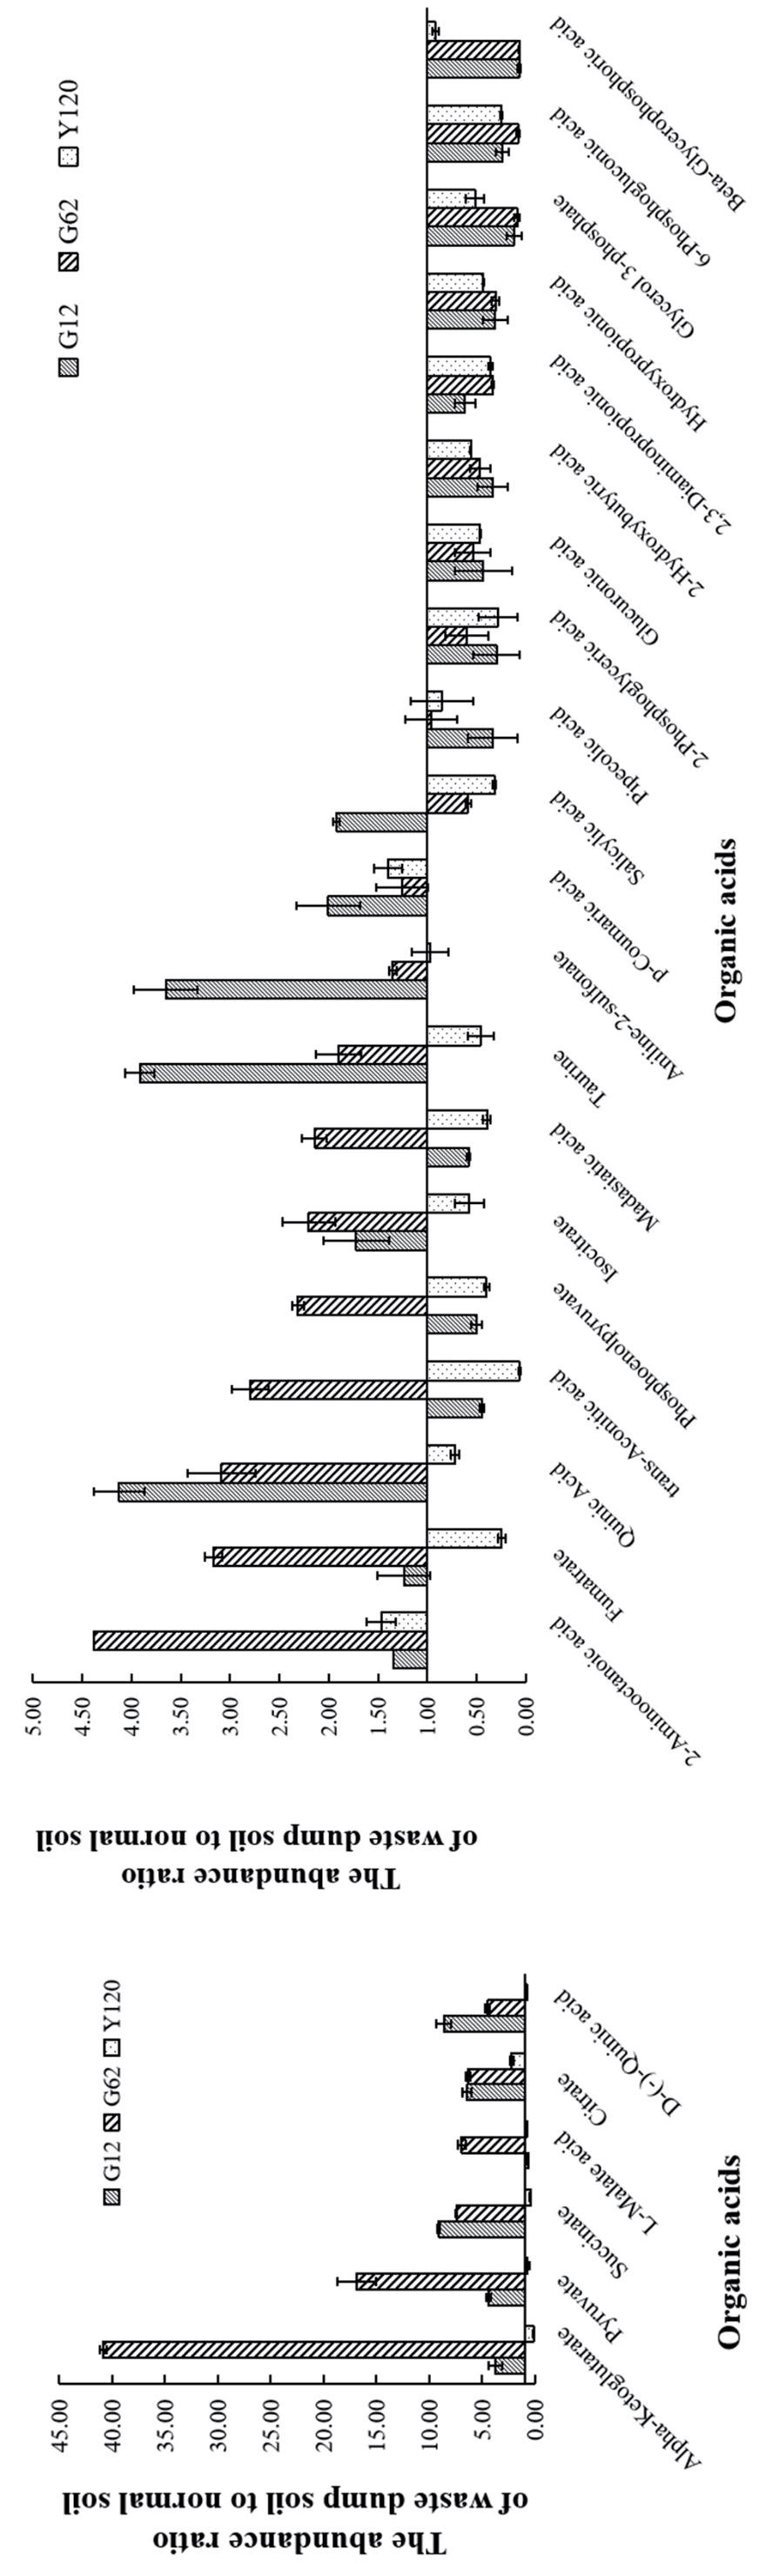
Fig. 6.
Abundance differences in saccharides in the three mulberry varieties planted in soil from waste dumps compared with normal soil.
Effects on the Secretion of Nucleosides and Their Derivatives
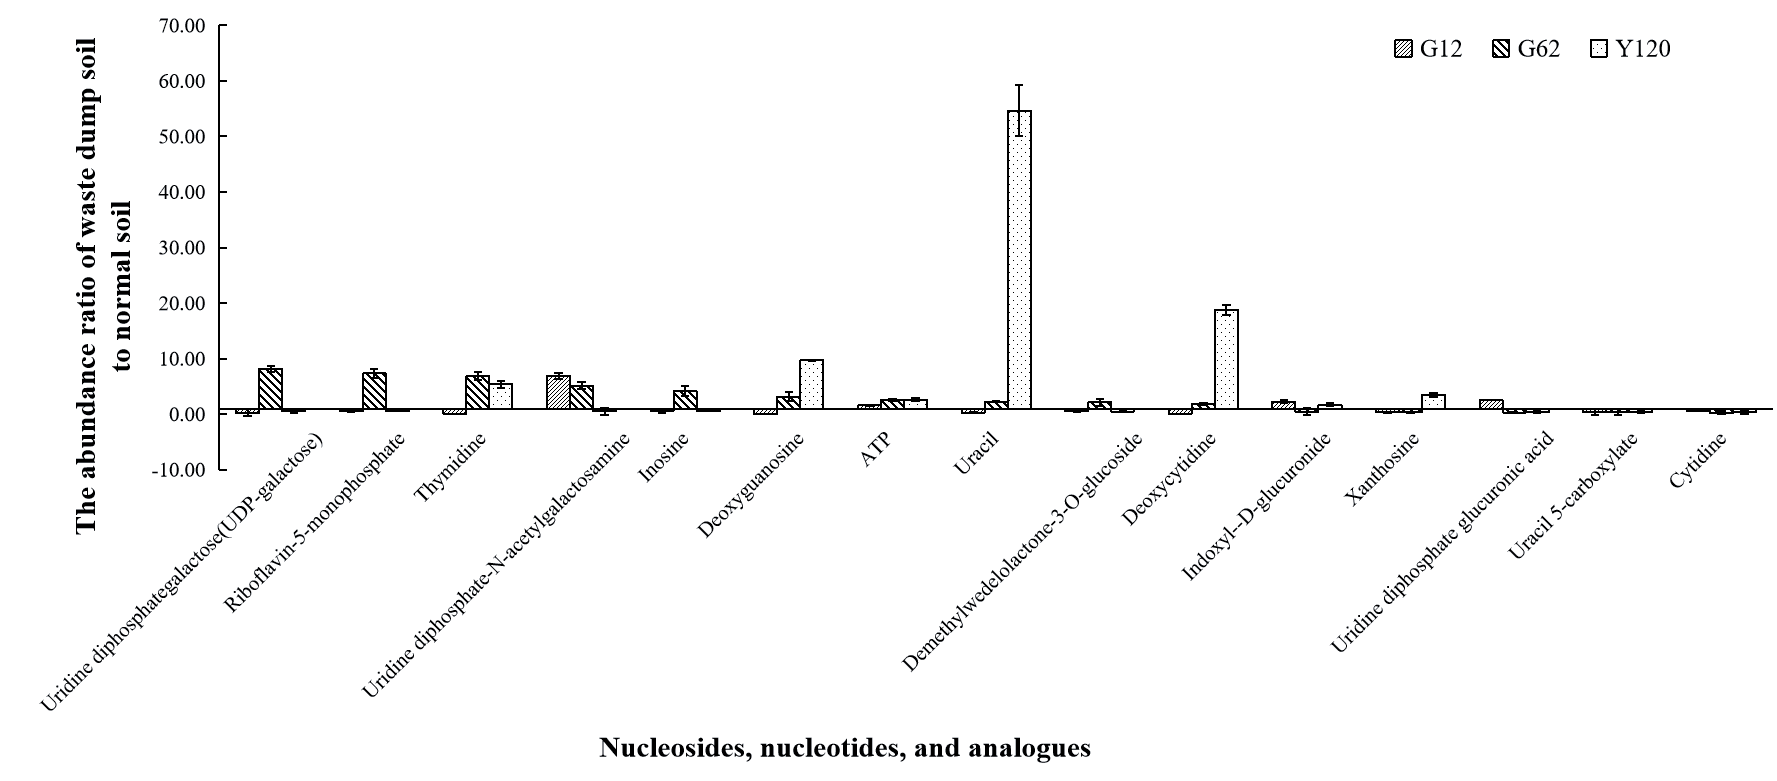
Compared with normal soil planting, the three mulberry varieties secreted uridine diphosphate-N-acetylglucosamine and no longer secreted three nucleosides (2‘-deoxycytidine 5‘-monophosphate (dCMP), N2, N2-dimethyl guanosine, and inosine triphosphate (ITP)) 60 days after planting in soil from waste dumps. There were significant differences in the content of 15 nucleotides secreted, including 10 nucleotides in G62, 4 nucleotides in G12, and 7 nucleotides in Y120 (Fig. 8). ATP levels significantly increased in all three varieties. Thymidine, deoxyguanosine, uracil, and deoxycytidine levels significantly increased in the best-growing G62 and medium Y120. Uridine diphosphate galactose, riboflavin-5-monophosphate, inosine, and demethylwedelolactone-3-O-glucoside significantly increased in G62 and decreased in the other two varieties. Thymidine, deoxyguanosine, uracil, and deoxycytidine may play an important role in reducing the toxicity of As elements in mulberry trees, making them more beneficial to the growth of mulberry shoots.
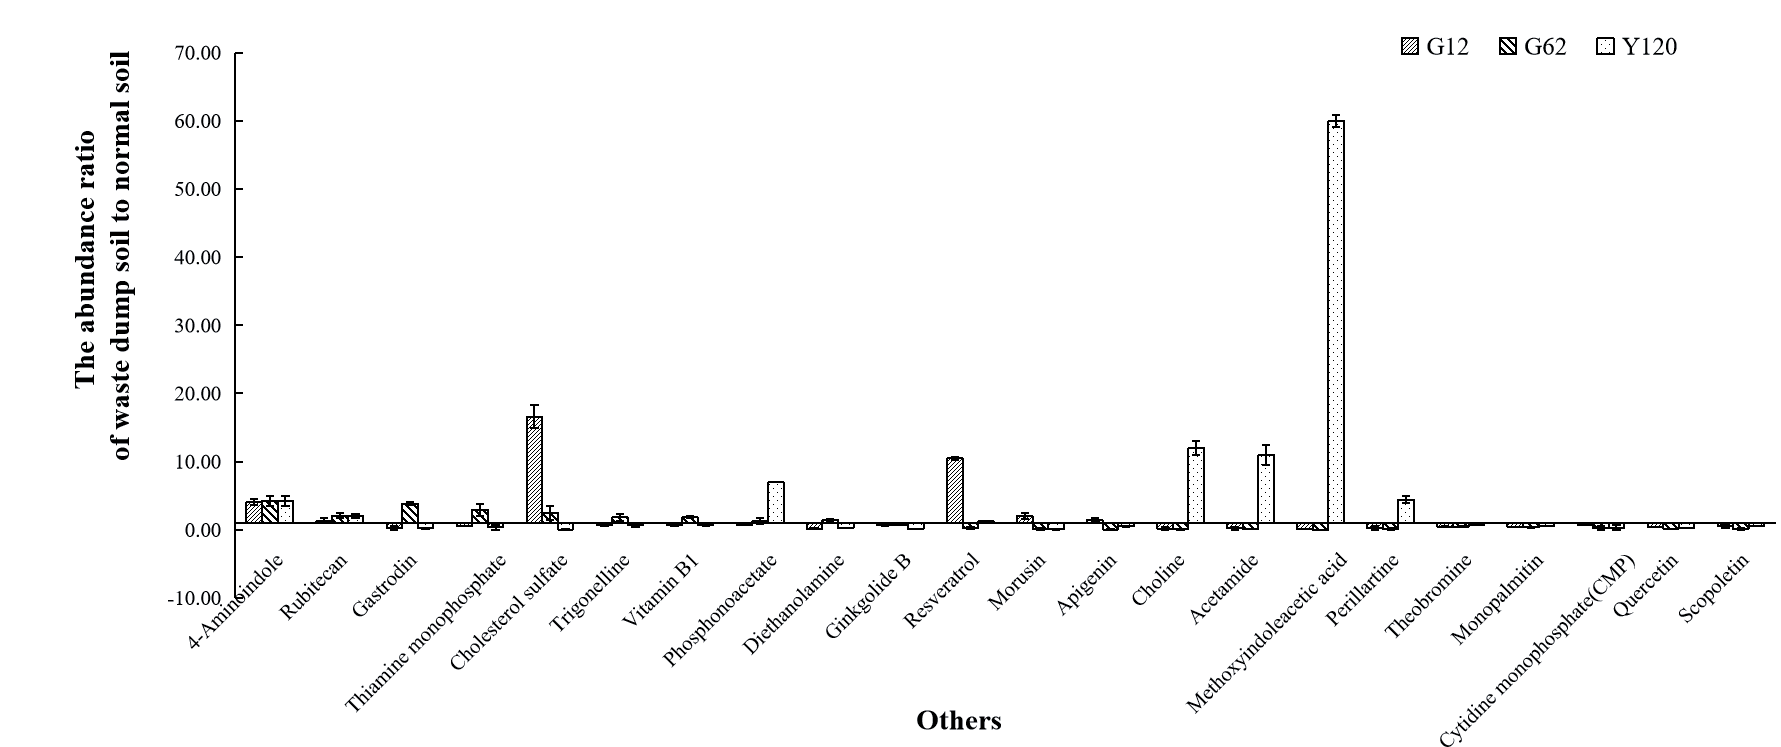
Effects on Secretion of Flavonoids, Polyphenols, and Other Compounds
Compared with normal soil planting, four compounds (dimethylallyl diphosphate, glutathione reduced, vitamin B2, and protirelin) were no longer secreted 60 days after planting in soil from waste dumps. 4-Aminoindole and rubitecan were significantly increased in the three mulberry varieties, especially 4-Aminoindole, which showed a significant increase (4.07–4.23) in the three varieties. 4-Aminoindole is an important intermediate of indole compounds and may be involved in the natural synthesis of growth regulators. It is worth noting that the secretion of cholesterol sulfate and resveratrol in G12 roots increased to 16.59 and 10.48 times that of normal soil growth (Fig. 9).
Discussion
Three mulberry varieties were planted in soil from waste dumps, which had a concentration 3.65 times higher than the standard value for agricultural land. The growth of the aboveground parts and roots was partially inhibited, but the degree of influence varied, suggesting that different mulberry varieties exhibited varying levels of As tolerance and detoxification. The excessive absorption of As elements by plants can inhibit their growth by interfering with their physiology and structure [20–22]. G62 exhibited the highest translocation coefficient and accumulated the highest amount of As in the body. Despite this, its growth was generally optimal, with more branches and leaves than in normal soil. Analysis of the root exudates revealed a significant increase in the types and concentrations of organic acids, sugars, and amino acids secreted by the roots. In contrast, G12 exhibited the poorest growth, leading to a decrease in both the type and quantity of the root exudates. Differences in As accumulation among different rice varieties are largely caused by variations in the quantity and composition of the root exudates [23]. The types and levels of organic acids, sugars, and amino acids increased with increasing As transfer capacity in the aboveground parts of the mulberry varieties. The high As content stimulated mulberry to initiate a series of stress-resistance reactions, leading to the synthesis of many organic acids, sugars, and amino acids to provide energy for supporting these reactions.
The higher variety and abundance of organic acids in G62 may be attributed to its ability to facilitate the transportation of As to the aboveground parts of the plant while reducing root toxicity. This enables plants to transport more As while maintaining healthy growth. This mechanism represents an adaptive strategy for mulberry plants to respond to As stress. Studies have shown that As stimulates the secretion of organic acids in the As hyperaccumulator Pteris vittata [24]. Organic acids in root exudates can form complexes with As ions in the soil, thereby affecting the migration of As [25]. Alpha-ketoglutarate (αKG) is an essential intermediate in the tricarboxylic acid (TCA) cycle [26]. It is involved in pleiotropic metabolic and regulatory pathways in the cell, including energy production, biosynthesis of certain amino acids, collagen biosynthesis, epigenetic regulation of gene expression, regulation of redox homeostasis, and detoxification of hazardous substances [27]. Citric acid acts as a bioregulator that participates in plant defense systems against abiotic stress [28]. It plays a significant role in As element tolerance [29]. Alpha-ketoglutarate and citric acid were significantly increased in the best-growing G62, which may be related to their involvement in the multi-pathway regulation of cells and the detoxification of As. Piperidine acid secreted by the root system of G12 with poor growth was significantly reduced. G62, with good growth, did not show a significant difference from normal growth, whereas Y120, with medium growth, rarely decreased. This may indicate that excessive As in the soil reduces the disease resistance of mulberry varieties, thereby affecting their growth. Studies have found that pipecolic acid (PIP) is a key signaling molecule that mediates the production of systemic acquired resistance (SAR) in plants. They can upregulate the expression of plant disease-resistance genes and induce the synthesis of plant disease-resistance metabolites, thereby enabling plants to produce SAR. Further correlation verification will be conducted in the future [30].
Compared with normal soil planting, the levels of two amino acids, lysine, and homoserine, significantly increased in G62 60 days after planting in an As-excess soil from waste dumps, which resulted in better growth and higher As accumulation. This may be attributed to the fact that G62 can reduce the transfer of As toxicity to plants, thereby minimizing its effect on mulberry growth. Studies have shown that amino acids are biological macromolecules and are important plant metabolites. In addition to maintaining the stability of macromolecular structures, participating in cell osmotic adjustment, and absorbing mineral nutrition, amino acids are also involved in plant responses to metal stress [31].
Soil with waste dump stress caused G62 roots to secrete various organic acids, including alpha-ketoglutarate, pyruvate, succinate, citrate, 2-amino octanoic acid, saccharides such as lactulose, trehalose, and sucrose, amino acids such as lysine and homoserine, nucleotides such as uracil, and 4-aminoindole. These secretions may contribute to the plant growth in soil from waste dumps. The types and levels of organic acids, sugars, and nucleosides secreted by the roots of G62 were higher than those secreted by G12 and Y120. This suggests that these compounds may play a more significant role in the response of mulberry plants to As stress. The cooperation of these three compounds may enable G62 to transport more As and reduce its toxicity to growth. Galactose metabolism, the pentose phosphate pathway, starch, and sucrose metabolism, and the citrate cycle (TCA cycle) were significantly affected in the G62 with improved growth. Moreover, the levels of galactose, citrate, and glucose in the metabolic pathway significantly increased. Galactose is a rich and essential sugar for plant biosynthesis [32]. The increase in galactose content in G62 may be related to its improved growth in soil from waste dumps. The sugar dextrose, amino acids threonine, isoleucine, leucine, nucleotide uracil, and lipid-like molecules, methoxyindoleacetic acid, secreted by Y120 roots in soil from waste dumps were abnormally higher than those in normal soil (25.76–122.34 times). This specific reason needs to be included in subsequent experiments to further verify its mechanism of Y120 adaptation to soil from waste dumps.
Mulberry is a medicinal and edible plant widely used in food, medicine, and animal feed. Many compounds in mulberry, such as polysaccharides, flavonoids, and DNJ, have important medicinal values. Soil with waste dump stress may lead to the secretion of important medicinal ingredients in mulberry roots, stems, leaves, and fruits, such as 4-Aminoindole. As an intermediate of indole derivatives, the synthesized indole acetic acid promoted mulberry rooting. The indole acetic acid derivative found in mulberry fruit may be beneficial for the treatment of human cervical cancer [33]. This significant increase may enhance the synthesis of medicinal components in roots, stems, leaves, and fruits. At the same time, it is worth noting that two components, cholesterol sulfate and resveratrol, which are beneficial for the treatment of human diseases, significantly increased root secretion in G12. Cholesterol sulfate is a steroid sulfate that plays an important physiological role in the human body. In recent years, it has been found to effectively alleviate ulcerative colitis [34]. Resveratrol is a phenolic compound produced by plants exposed to unfavorable conditions. It can inhibit oxidative stress by reducing free radical content, reducing the production of lipid peroxides, and enhancing the activity of antioxidant-related enzymes. Resveratrol has antioxidant, anti-inflammatory, anti-tumor, and neuroprotective effects [34–37]. The increase in the medicinal components of these compounds may indicate that they also help mulberry trees enhance their resistance to As stress. Studies have shown that toxic element stresses, such as Cu, Pb, Cr, and As, can directly produce reactive oxygen species in plants. Excessive production of reactive oxygen species can cause cellular damage, but plants can use defense mechanisms to mitigate these effects [38, 39]. However, As stress can also stimulate mulberry roots to enhance the secretion of vital medicinal components in their plants. These components can then be transported to the relevant tissues and organs, thereby boosting the effectiveness of medicinal ingredients. This study will provide ideas and ways to promote the targeted production of medicinal ingredients in mulberry through the excavation and utilization of abiotic stress and related genes.
In this study, the content of As in the aboveground parts of the three mulberry varieties was within the standard range for their use as feed (GB 13078-2017). Therefore, the results of this study provide important insights into the restoration and utilization of As-exceeding mine soils. The results of this study provide a basis for identifying root exudates that enhance As adsorption by mulberry roots. It can also help in identifying mulberry root exudates that can thrive in soil from waste dumps, thereby improving the remediation of As pollution in mine soil. By modifying the type and composition of mulberry root exudates, this study aimed to support the healthy growth of soil and ensure human safety.
Conclusions
This experiment confirmed that As pollution can affect mulberry metabolites. Therefore, we can screen out metabolites that may contribute to the growth of plants in As pollution. Through metabolomics studies, we found that a variety of metabolites in mulberry root exudates changed. Among them, G62 grew best, and the types and abundances of organic acids, sugars, nucleosides, and their derivatives secreted by its roots were significantly higher than those of G12 and Y120. Soil with waste dump stress significantly increased the secretion of several organic acids such as Alpha-Ketoglutarate, Pyruvate, Succinate, Citrate, 2-Aminooctanoic acid, saccharides such as Lactulose, Trehalose, Sucrose, and Dextrose, amino acids such as Lysine and Homoserine, nucleosides such as Uracil, and 4-Aminoindole in G62 roots. It may help G62 to better adapt to soil from waste dumps and promote its growth. In this study, the content of As in the aboveground parts of the three mulberry varieties was within the standard range for their use as feed (GB 13078-2017). Therefore, the results of this study provide important insights into the restoration and utilization of As-exceeding mine soils. The results of this study provide a basis for identifying root exudates that enhance As adsorption by mulberry roots. It can also help in identifying mulberry root exudates that can thrive in soil from waste dumps, thereby improving the remediation of As pollution in mine soil. By modifying the type and composition of mulberry root exudates, this study aimed to support the healthy growth of soil and ensure human safety.

