


Introduction
Nectar and pollen are the natural feed of the honey bee (Apis mellifera L.) colony. A yearly amount of 80 kg of honey and 20 kg of pollen is consumed by a honey bee colony [1]. Pollen is more crucial than nectar because it provides the nutritional requirements for developing bees [2, 3]. Honey bees collect pollen mainly to meet their requirements of protein, lipids, fatty acids, mineral elements, antioxidants, and vitamins [3–6]. Protein plays a critical role in the honey bees’ lives [7]. Protein normally found in pollen is necessary for brood production. Nurse bees must consume pollen to develop the hypopharyngeal glands to secrete the royal jelly required to feed young larvae and queens [8, 9].
The quantity and quality of pollen available to a bee colony is a limiting factor in beekeeping. During a dearth period as a result of a decline in pollen gathering activity, the brood rearing declines and the colony population size decreases, so artificial feeding with pollen substitutes is necessary to enhance the activities of honey bee colonies and for sustaining brood rearing in honey bee colonies [7, 10]. Pollen substitutes are well accepted by bee workers during the absence of natural pollen [7, 11]. Pollen substitutes must have nutritional values and be free from anti-nutritional factors [8, 11, 12]. A good diet should be acceptable to the bee workers and meet the nutrients required for colony growth and development, bee health, and colony production [12, 13]. The honey bee workers cannibalize the young brood in malnourished colonies and new broods are not produced [14]. Furthermore, deficiencies in colony nutrition may be considered a factor in recent honey bee colony losses [15].
A beekeeper may feed colonies on pollen substitutes or pollen supplements containing nutrients that are essential to their health to stimulate brood rearing in the late winter or early spring or to relieve dietary stress when pollen from blooming plants is scarce or has a marginal nutritional value [10, 12]. Many diet formulations have been developed by combining different ingredients and examined for beekeeping all over the world [11, 16–20]. Pollen substitute has the ability to enhance the performance of honey bee colonies [7, 11].
Colony performance and productivity have been affected by many factors including availability of nectar and pollen flora [9, 21], subspecies of honey bees [22], colony population size [23, 24], feeding pollen substitutes [8, 11, 18–20], season [22, 23], age of the comb [25–28], and weather factors [22, 24].
The sustaining of colony strength during winter and dearth periods is a worrying problem for beekeepers around the world. The study may hypothesize that providing honey bee colonies with a protein diet during winter and spring has a high ability to maintain the adult population size and enhance the colony activities. So, the present study aimed to evaluate the efficiency of three pollen substitutes in maintaining the colony strength during winter and improvement of colony performance and honey yield during spring.
Material and Methods
Study Area
The experiments were conducted at a private apiary in Desouk (31°8′32″ N, 30°38′42″ E), Kafrelsheikh province during the winter and spring seasons of 2022/2023. In addition to the minor nectar and pollen flora, Faba bean (Vicia faba L.) and flax (Linum usitatissimum L.) were the most important plants for honey bees during winter, and Egyptian clover (Trifolium alexandrinum L.) was the predominant nectar and pollen source during spring in the experimental area.
Experimental Colonies
The varroa mite, Varroa destructor (Anderson and Trueman), was controlled in the experimental apiary before the beginning of the experiment using the oxalic acid vaporization method. Twenty colonies (each of 7 combs) of Carniolan hybrid honey bee (Apis mellifera carnica Pollmann) of the same strength were divided into four groups (five colonies for each treatment). Three groups (each of 5 colonies) were fed protein diets as pollen substitutes; meanwhile, the 4th group was deprived of proteinous feeding (control). One liter of sugar syrup (1:1) was provided to each colony at 7-day intervals during the nectar scarcity periods. The experiments were conducted during the winter season of 2022/2023 and during the spring season of 2023.
Experimental Diets
The components of the tested diet formulations were as follows: 30 g peeled white lupine (Lupinus albus) flour + 20 g brewer’s yeast + 20 g casein milk powder + 20 g honey + 10 g sugar powder (diet 1), 30 g fenugreek (Trigonella foenum-graecum) flour + 20 g brewer’s yeast + 20 g casein milk powder + 20 g honey + 10 g sugar powder (diet 2), and 30 g defatted soybean (Glycine max) flour + 20 g brewer’s yeast + 20 g casein milk powder + 20 g honey + 10 g sugar powder (diet 3). The diet ingredients were mixed to make a paste and placed on waxed paper to prevent moisture loss.
Chemical Composition of Diets
A sample of each diet was used to estimate the proximate analysis of the diet. A sample of 2 g was dried at 105°C until the constant weight to estimate the content of moisture. The methods described by AOAC [29] were used to estimate the crude protein content, crude lipid content, crude fibers, and ash content. The Kjeldahl method estimate was used to determine the nitrogen content by using a sample of 0.5 g of diet, the total nitrogen was converted to crude protein by multiplication of the 6.25 factor. The Soxhlet apparatus was used to extract the fat content of a sample of 2 g diet using petroleum ether (40–60ºC) for 6 hrs. Ash content was determined by incinerating a sample of 2 g diet in a muffle furnace at 550°C. A sample of 2 g diet was digested for gravimetric determination of the crude fibers as a residue that remained after the alkaline and acid digestions. The available carbohydrates were calculated by subtracting crude fats, moisture, crude fibers, ash, and crude proteins from 100. All estimations were performed in triplicate.
Feed Consumption
The diets were offered freshly on a paste form to the colonies directly over the brood nest at a rate of 100 g/colony/week and changed weekly by new pastes. The unconsumed diets were collected and weighted to calculate the weekly feed consumption of each diet.
Colony Activities
The areas (square inches) of stored pollen and worker-sealed brood were measured at 12-day intervals using a plastic sheet (the same area as an empty standard frame) divided into square inches. By the end of each season, the number of combs covered with bees/ colony was recorded to determine the colony population size. Bee population size per colony was counted as one comb well covered with bees on the two sides equals 2000 bees [30]. By the end of the flow seasons of Egyptian clover (Trifolium alexandrinum L.) at the beginning of June, the honey yield was determined by the difference between the weight of honeycombs before and after honey extraction [22].
Statistical Analysis
The normality of the data was tested using the Shapiro-Wilk normality test, which indicated the normal distribution of the data. Therefore, the original data were analyzed. The data of each season were statistically analyzed separately. The differences between the treatments were tested by one-way analysis of variance (ANOVA). The PROC GLM function in SAS version 9.1 [31] was used for data analysis. The treatment means were compared using Tukey’s HSD post-hoc test. Pearson correlation coefficients between feed consumption, stored pollen area, worker-sealed brood area, colony population size, and honey yield during the winter and spring seasons were estimated.
Results and Discussion
The chemical composition of the experimental diets is presented in Table 1. The highest contents of moisture (19.09%), crude fibers (6.35%), and crude fats (5.91%) were detected in diet 1. The highest contents of crude protein (23.07%) and available carbohydrates (46.15%) were detected in diet 3. The highest ash content (6.03%) was detected in diet 2. Meanwhile, the lowest contents of protein (21.27%) and moisture (18.53%) were detected in diet 2. The lowest contents of crude fibers (4.13%), crude fats (3.53, and ash (4.12%) were detected in diet 3. The lowest content of available carbohydrates (41.71%) was detected in diet 1. The experimental diets contain the same amount (70%) of all ingredients including 20% brewer’s yeast, 20% casein milk powder, 20% honey, and 10% sugar powder, and differed in 30% of diet components which represented 30% peeled white lupine flour in diet 1, 30% fenugreek flour in diet 2, and 30% defatted soybean flour, so the composition differences among diets should be related to the different 30% (lupine, fenugreek, and soybean) of each diet. However, the impacts of diets on colony activities resulted from the all components of each diet. The contents of protein and lipids in the experimental diets were relatively similar to protein and lipids in bee pollen from major pollen plants [2, 3, 6, 32]. Meanwhile, the contents of fibers and mineral elements in the experimental diets were higher than those in bee pollen [3, 33–36]. The chemical composition of the experimental diets confirms the possibility of using any of them as a good substitute for bee pollen.
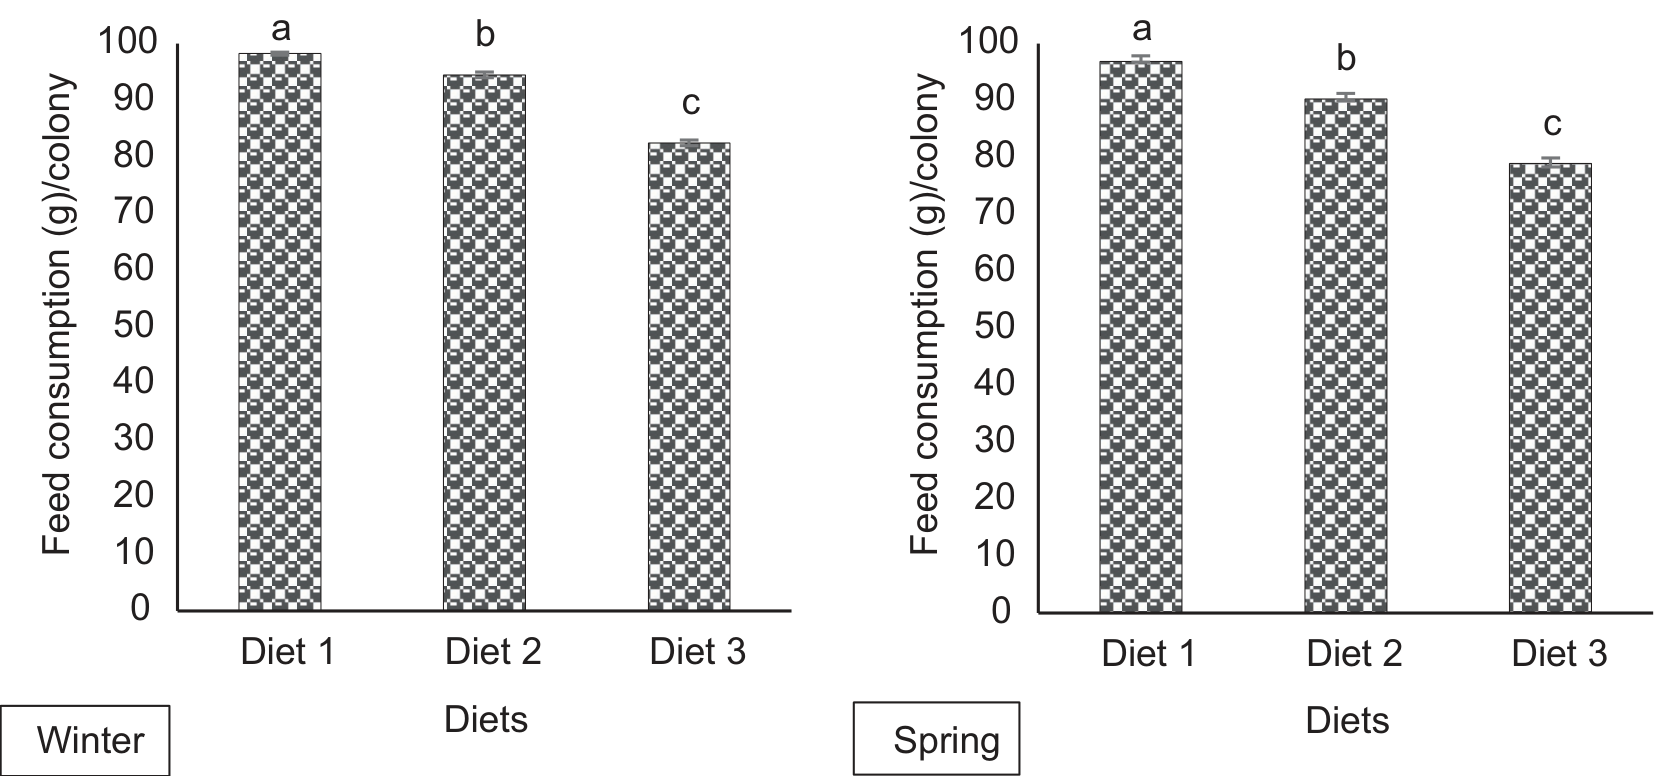
Data illustrated graphically in Fig. 1 show that the largest amount of consumed feed was from diet 1 (30 g peeled white lupine (Lupinus albus) flour + 20 g brewer’s yeast + 20 g casein milk powder + 20 g honey + 10 g sugar powder), while the lowest amount was consumed from diet 3 (30 g defatted soybean (Glycine max) flour + 20 g brewer’s yeast + 20 g casein milk powder + 20 g honey + 10 g sugar powder) during winter and spring seasons. Colonies fed on diet 1 consumed 98.22 and 96.84% of the provided diet compared to 94.48 and 90.25 % for colonies fed on diet 2, and 82.50 and 78.91 % for colonies fed on diet 3 during the winter and spring seasons, respectively. The amount of consumed feed was significantly (P < 0.01) varied depending on the ingredients of the diet as well as the season. Diet 1 had the best palatability may be due to the ingredients of the diet which affect the attraction of bees for feeding. In addition, the variations in feed consumption might be related to the size of the bee population in colonies. A large population size colony consumes feed more than a small population size colony. A significant positive correlation (r = 0.87 – 0.89; P < 0.01) between the amount of feed consumption and the adult population size in the colonies was detected (Table 2). The current results confirm the findings obtained by Israr et al. [7] and Taha [11] who detected a significant positive correlation between feed consumption and colony strength.
Table 2.
Correlation coefficients between feed consumption and stored pollen, worker-sealed brood area, adult population size, and honey yield during the spring season.
Fig. 1.
Amount (g)/colony of weekly consumed feed during the winter and spring seasons. Different letters above the bars indicate a significant difference (P < 0.01) according to Tukey’s test.
Data in Fig. 2 describe the stored pollen area in the combs during the winter and spring seasons. Significant (P < 0.01) differences were detected between the fed and unfed colonies and among the tested diets. In comparison with the unfed colonies, feeding colonies on protein diets during the winter and spring seasons increased the area of stored pollen by 65.20 and 47.34 % for diet 1, 52.03 and 31.08 % for diet 2, and 37.10 and 16.20 % for diet 3, respectively. The current results agree with those obtained by Taha [11, 37], Islam et al. [19], and Pokhrel et al. [38] who found that feeding colonies with pollen substitutes during spring significantly increased the area of stored pollen. The variations in stored pollen area were correlated (r = 0.85 – 0.94; P < 0.01) to the diet consumption that leads to a high rate of brood rearing, and subsequently number of foragers, that collected pollen from pollen flora. The colony population size was significantly positively correlated (r = 0.92 – 0.95; P < 0.01) with the area of stored pollen. A significant (P < 0.01) variation in stored pollen area was detected between the winter and spring seasons. This variation could be correlated to the availability of the major pollen flora during the two seasons [11, 21, 22, 39].
The worker-sealed brood area during winter and spring seasons was illustrated in Fig. 3. Worker-sealed brood area was significantly (P < 0.01) influenced by feeding colonies with protein diets. Pollen substitutes are provided to honey bee colonies in early winter to maintain the strength of colonies and during late winter and early spring to enhance the colonies’ building up. In addition to the colony strength, brood production, and population growth in the colonies are affected by queens’ quality, the subspecies of bees, and the availability of nectar and pollen sources [22]. The current study was conducted in one location, the queens of all colonies are sisters, brood areas, feed storage, and colony strength were relatively similar in all colonies, so all parameters are constant regardless of the artificial nutritional factors. Also, significant (P < 0.01) variations in worker-sealed brood areas among colonies fed the three diets were detected. Colonies provided with diet 1, diet 2, and diet 3 produced worker broods more than the unfed colonies by 29.03 and 25.00%, 25.81 and 22.50%, and 17.74 and 12.50% during the winter and spring seasons, respectively. The current results confirm the results reported by Israr et al. [7], Islam et al. [19] Ullah et al. [40], and Topal et al. [41]. Pokhrel et al. [38] fed colonies 3 weeks on sugar candy and pollen substitute in May. They obtained higher (158.80%) brood production than brood production in June. Also, Matilla and Otis [10] reported that colonies started rearing broods earlier when supplemented with pollen or a pollen substitute in the spring, and a large adult population was produced by late April or early May. Strong positive correlations were detected between brood area and feed consumption (r = 0.90 – 0.96; P < 0.01), and stored pollen area (r = 0.96 – 0.99; P < 0.01) (Table 2). The current results confirm the results obtained by Taha [11] regarding the correlation with feed consumption, and by Taha and Al-Kahtani [22] for the correlation with an area of stored pollen. The significant (P < 0.01) differences in brood production between winter and spring seasons could be related to adult population size in the colonies which correlated with the area of stored pollen that is affected by the availability of nectar and pollen flora [11, 23].
Fig. 2.
Impact of feeding protein diet on stored pollen area (square inches)/colony during the winter and spring seasons. Different letters above the bars indicate a significant difference (P < 0.01) according to Tukey’s test.
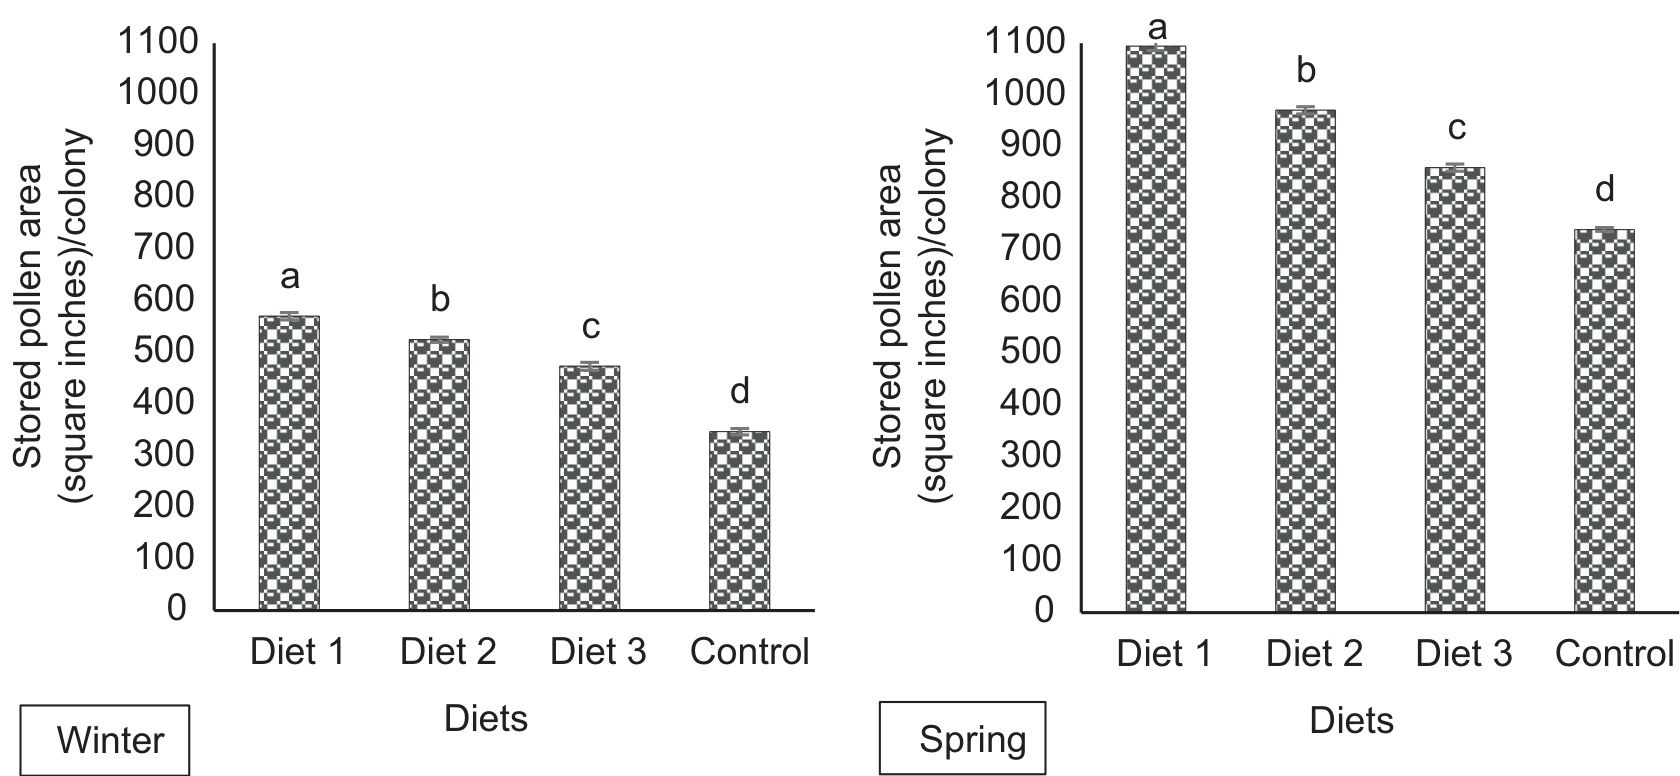
Fig. 3.
Impact of feeding protein diet on the area (square inches) of worker-sealed brood/ colony during the winter and spring seasons. Different letters above the bars indicate a significant difference (P < 0.01) according to Tukey’s test.
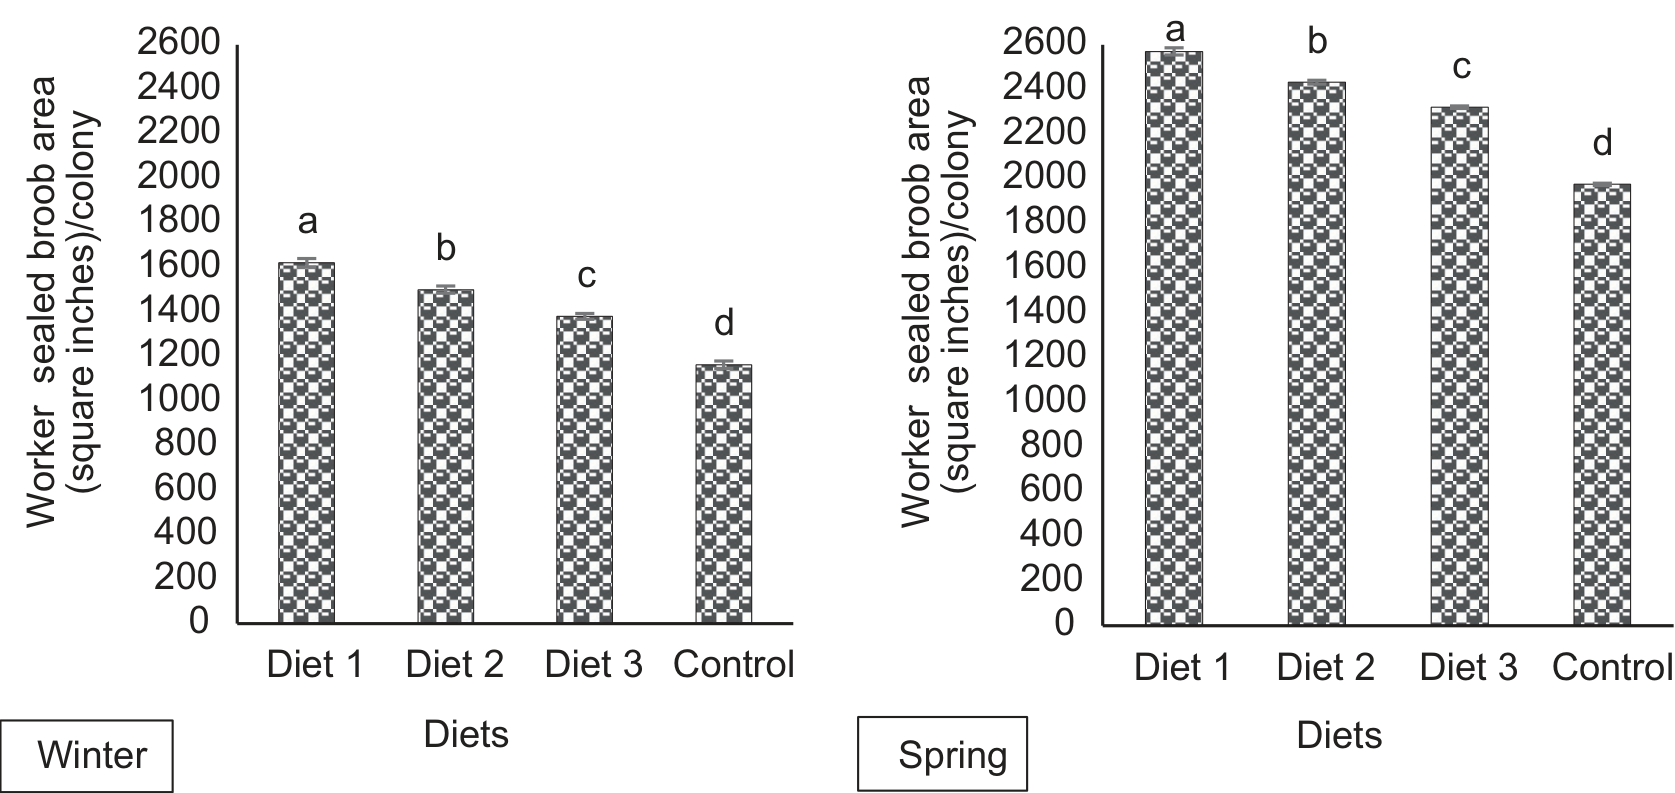
Fig. 4.
Impact of feeding protein diet on colony population size during the winter and spring seasons. Different letters above the bars indicate a significant difference (P < 0.01) according to Tukey’s test.
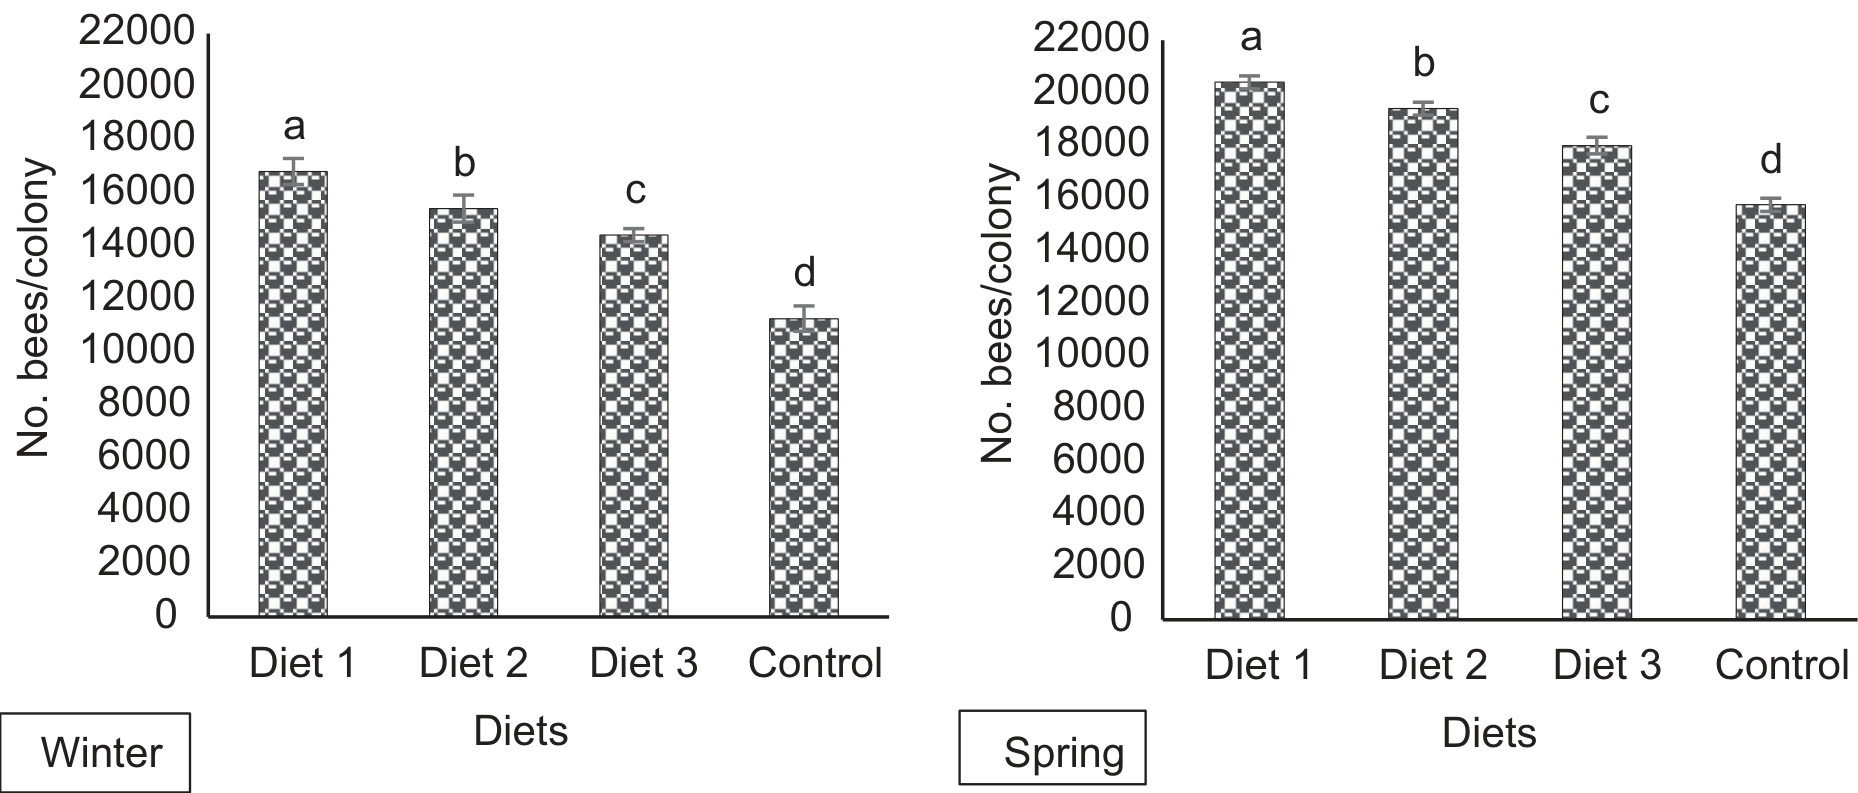
Fig. 5.
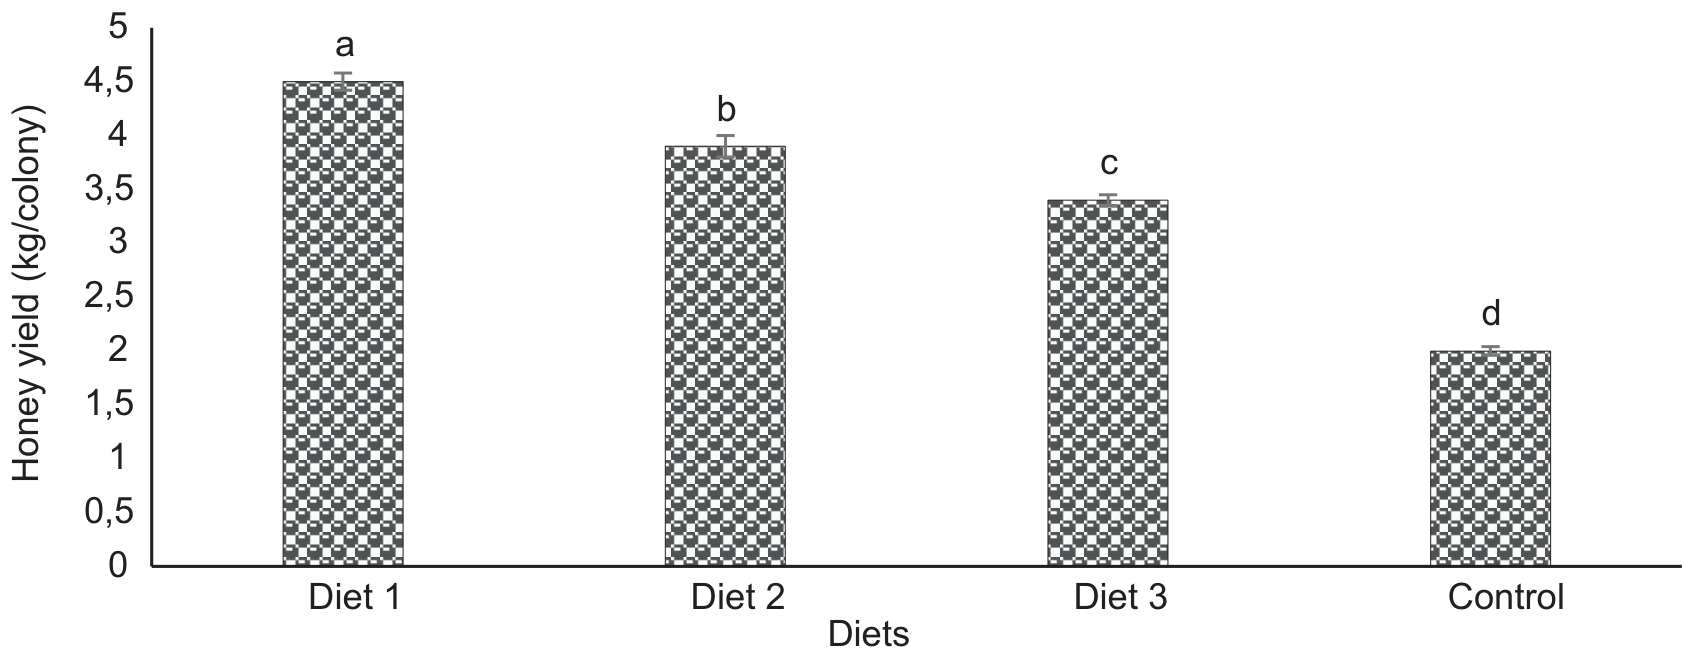
Impact of feeding protein diet during spring on honey yield (kg/colony). Different letters above the bars indicate a significant difference (P < 0.01) according to Tukey’s test.
As illustrated in Fig. 4 the adult population size in a colony was significantly (P < 0.01) affected by feeding colonies with protein diets. Moving colonies to a rich nectar and pollen location increased the number of reared bees by 33.33% more than colonies in an apiary located in a poor-flora area [30]. Feeding colonies of honey bees on protein diets raised the adult bee population size by 32.26 and 28.75 % for diet 1, 25.81 and 22.50 % for diet 2, and 16.13 and 15.00 % for diet 3 more than the unfed colonies during winter and spring seasons, respectively. These results agree with the findings obtained by Israr et al. [7], Taha [11], and Topal et al. [41]. Feeding colonies with a protein diet and candy in May for three weeks raised the bee population size by 15.00% more than in June [38]. In addition, feeding colonies additional pollen or pollen substitutes during the spring increased the adult population by 12200 workers/colony in May compared to colonies in winter [10].
Data illustrated in Fig. 5 display that there were significant (P < 0.01) differences between honey yield harvested from the fed and unfed colonies, and among colonies fed the experimental diets during the spring season. Egyptian clover (Trifolium alexandrinum) honey was harvested near the end of spring. Colonies fed on protein diets produced significantly more honey than the unfed colonies by 125.00, 95.00, and 70.00% for diet 1, diet 2, and diet 3, respectively. Colonies fed on diet 1 produced honey more than colonies fed on diet 2 and diet 3 by 15.38 and 32.35%, respectively. The current results confirm the findings previously obtained by Islam et al. [19], Matilla and Otis [10], Pokhrel et al. [38], and Ullah et al. [40] who observed that feeding honey bee colonies with protein diets raised honey yield. Taha [11] reported that providing colonies with a diet consisting of 40% brewer’s yeast + 40% defatted soybean flour + 10% skimmed powder milk + 10% honey produced 202.86% honey yield of the unfed colonies. Feeding colonies on protein diets leads to colony superiority in honey production that resulted from collecting more nectar from major nectar flora by a large adult population that correlated (r = 0.99, P < 0.01) with the high rate of worker brood rearing. The high population of workers was strongly correlated (r = 0.94, P < 0.01) with the area of bee bread in the colonies (Table 2). Also, honey yield was significantly positively correlated with feed consumption (r = 0.94, P < 0.01) and stored pollen area (r = 0.96, P < 0.01). Relatively similar results were recorded by Taha and Al-Kahtani [23] who decided that the honey yield produced from two weak colonies was significantly lower than the honey yield produced from one strong colony.
Significant (P < 0.01) differences in stored pollen area, worker-sealed brood area, and colony population size were detected between the winter and spring seasons. The variations between the two seasons were correlated to the meteorological factors [22] and the availability of nectar and pollen plants [11, 21, 22, 42, 43], also the cultivated area of the major nectar and pollen flora, the amount of nectar secretion of plants, and sugar concentration in nectar during each season had considerable effects [30].
Conclusions
Supplying honey bee colonies with a protein diet during winter and early spring, or scarcity of pollen from blooming plants was a vital requirement in beekeeping. From the obtained results, diet 1 (30 g peeled white lupine flour + 20 g brewer’s yeast + 20 g casein milk powder + 20 g honey + 10 g sugar powder) was the most preferred diet for honey bee colonies. Colonies fed on diet 1 exhibited the best performance in storing pollen, worker brood rearing, colony growth, and honey production. Diet 1 could be recommended as a good protein diet (pollen substitute) during the winter and spring seasons to sustain the brood production and strength of the colonies and improve colony productivity.

