

Introduction
The unusual shift in the natural environmental conditions because of growing population, elevated air and soil contamination, ecosystem toxicity from heavy metals, exhaustion of soil attributes, and worldwide climate variability has substantially influenced the potential of plants to respond to evolving climatic circumstances [1]. These alterations make agro-productivity systems vulnerable to fluctuating ecological conditions. Such hostile climatic events can cause harm to the physiological processes that plants undergo, known as stresses [2]. Environmental perturbations that limit plant development and agricultural productivity beneath the threshold point are known as abiotic stresses. These include extreme temperatures, metallic toxicities, water scarcity, soil salinity, and nutrient imbalance.
Cadmium is recognized as one of the most hazardous metal components in polluted agricultural lands due to its extensive contamination, considerable mobility, and extreme toxicity to human beings, livestock, and economic crops [3]. Both acute and long-term disclosure to Cd can lead to serious consequences, such as serious impairment and suppression of plant physiological activities, excessive production of nitrogen species and reactive oxygen species within cells that could also serve as harmful substances regulating an oxidative/ nitrosative burst that can lead to an intensified process of senescence in plants, stunted growth, and ultimately plant decease [4]. Cd causes oxidative damage at the cellular level by serving to supply electrons to molecular oxygen, which in turn stimulates the formation of detrimental reactive oxygen species (ROS) [5]. Plants use an array of defense mechanisms to avert Cd toxicity, such as metal phytochelatin and retention, as well as the activation of ROS neutralization and combating systems involving both antioxidants (enzymatic and non-enzymatic) [6].
Sunflower (Helianthus annuus L.), an annual plant species, can accrue significant levels of U and Cd within its tissues [7]. One of its main contributions as an industrial product is its dry biomass. It has important agronomic traits like soil variability and resilience to intense climate variability [8]. Its sensory, nourishing, and functional qualities make it a highly desirable protein source for the ingestion of humans [9]. The sunflower is recognized as a crucial plant species for use in phytotechnology due to the fact that it has a significant capacity for tolerance among heavy metals [10]. Previous research has shown that arsenic (As) and cadmium (Cd) drastically decrease the seed germination rate. Its capability to transport heavy metals from beneath the soil into the consuming parts of plants through the roots is quite promising [11]. Zinc (Zn) is an essential component of several kinds of enzymes, and it plays an integral part in the functioning role of enzymes to control a variety of cellular functions [12]. In addition to having more similarities with cadmium, zinc, which is a divalent ion, may compete with cadmium for binding sites in the soil and on the root surface, which may affect the translocation of cadmium in plants [13]. Zn application may reduce the Cd absorption from soil and perform a vital function in mitigating the noxious effects of Cd in plants by modulating a number of potential mechanisms, like minimizing the impact of restricted plant growth and regulating the process of Cd absorption and its relocation. However, these are only the basic effects of zinc application under cadmium stress. Furthermore, zinc application resulted in improved plant nutrient status, enhanced photosynthetic rate, activated antioxidant defense mechanisms, and lowered production of ROS, and at the same time also proved to be an effective strategy to reduce the harmful effects caused by cadmium on plants [14].
The objective of the present research was to find out how zinc application impacted the morpho-physiological and biological attributes of sunflowers under contexts of cadmium stress and contamination. The present study will assess the positive effects of zinc application on the overall botany of sunflower plants.
Experimental
The existing experiment was carried out in a pot at the University of Agriculture Faisalabad, postgraduate agriculture research station (Latitude: 31.383230648, Longitude: 72.9948305931) during the summer season of 2021 in order to investigate the possible role of zinc in alleviating Cd stress in sunflower. A sunflower variety “FH-516” was obtained from the Ayub agriculture research station and sown in a pot (having dimensions 25 cm × 22 cm × 20 cm) containing an 8 kg clay soil mixture. A total of 27 pots were taken for an experiment that was organized in accordance with a two-factorial experimental layout and three replications under a completely randomized design. In each pot, 10 healthy seeds were sown up to 2 cm depth. One day before sowing, irrigation was done with tap water. These pots were 2-holed at the lower side (covered with muslin cloth) to prevent the accumulation of excess water. Regular watering was maintained, and one week after seeding, thinning was performed by maintaining four plants in every pot for further inspection. A very small quantity of urea was applied before the thinning of seedlings for better crop growth. Three levels of cadmium (0, 40, and 80 ppm) and three levels of zinc (0, 50, and 100 ppm) were used in this experiment, and the source of Cd and Zn was cadmium nitrate and zinc sulfate, respectively. These were taken from the laboratory of the Botany Department UAF-community college PARS in a required amount, and solutions were made in one-liter distilled water and applied exogenously to specific plants after 25 days of germination.
Morphological Parameters
After three weeks of supplying treatments, two plants were harvested from every pot. Plants were carefully uprooted and cleansed using ordinary tap water. Measurements were taken for morphological, biochemical, and yield attributes.
The fresh weight of the root and shoot samples was recorded immediately in a laboratory using a weighing scale. After that, the samples were stored in an oven at a temperature between 65 and 70ºC for a period of two weeks in order to investigate the dry weight of the root and shoot samples. The root length, leaf length, and shoot length of each plant were recorded on a measuring scale, and the leaf area of each plant was measured using a leaf area meter.
Chlorophyll Contents
For the purpose of determining chlorophyll a, chlorophyll b, the a/b ratio, and carotenoids, the technique developed by Arnon was used [15]. Chlorophyll a, chlorophyll b, and carotenoids were assessed by measuring the absorbance of 0.1 grams of fresh leaf sample that was put in 80% acetone. The absorbance was measured at 663, 645, and 480 nm, respectively.
The following formulae were used to calculate the chlorophyll content quantitatively;
Acar = OD480 + 0.114 (OD 663) - 0.638 (OD 645)
Em = 2500
V = Volume of the extract (ml)
W = Weight of fresh leaf tissue (g)
Flavonoids
For determining flavonoids using the method proposed by Chang [16], 0.1 grams of fresh leaf material was taken and homogenized with 2 milliliters of a solution containing 80 percent acetone. Following this, 4 milliliters of distilled water were added to 1 milliliter of extracted material, and at 510 nanometers, the material absorbance was measured by using a spectrophotometer.
Anthocyanin
To determine the anthocyanin content of sunflower leaf material, using the Strack and Wray method [17], fresh leaf material weighing 0.1 grams was ground using 1 milliliter of acidic methanol. Afterward, the mixture was heated up to a temperature of 50 degrees Celsius for one hour, and then it was filtered. A spectrophotometer was used at a wavelength of 535 nm to determine the absorbance of the substance.
Ions (Na+, Ca2+, K+) Determination
For digestion of dry samples, freshly prepared nitric acid (HNO3) and hydrochloric acid (HCl) together form a combination with a ratio of 3:1 (aqua regia) was used. For two hours, 1 gram of plant root and shoot samples were heated with 2 ml of aqua regia in a crucible at the flame, till all plant material was completely digested and black ash was obtained. After that, the ash was ground up into a high-quality powder and mixed with a 10% solution of nitric acid. After one hour, this sample solution was filtered and stored in airtight sampling bottles for the determination of Na+, K+, and Ca2+ of the root and shoot, according to the Vázquez method [18].
Seed Oil Contents (%)
Following the ginning, seed samples of sunflower plants were treated with acid and then dried for 24 hours at 40ºC in the oven. The seed husk was gently crushed using a nutcracker. The oil content of the embryo was then determined by Soxhlet extraction [19]. It can be inaccurate to describe the composition of sunflower seeds using percentages, particularly when the weight of the seeds varies. As a result, the embryo oil index was calculated to express composition based on weight rather than percentages. The oil content of the embryo was quantified both as a percentage of its weight (referred to as embryo oil percentage, EO%) and as a weight in milligrams (known as embryo oil index, EOI).
Embryo oil index (weight of oil in 100 embryos) = embryo oil % × acid-delinted, seed index/100
Protein Contents
Proteins were estimated by using the Brad Ford method [20]. After grinding the sample, 0.2 grams of phosphate buffer with a pH of 7 were added to 10 milliliters of the solution. Afterward, the extract was filtered. Test tubes were filled with 1 milliliter of the plant sample and 1 milliliter of the extract. After allowing the test tubes to be kept at room temperature for half an hour, 0.5 milliliters of the Folin reagent were added. Again, they were kept at room temperature, and 5 mL of distilled water was added. Measurement of absorbance was performed at a wavelength of 620 nm. A blank was prepared by taking 1 mL of Buffer and 2 mL of Bradford.
Yield Attribute
The number of seeds of each flower was calculated through a simple counting method, and mean values were calculated, respectively. The weight of 100 completely grown seeds was measured using a weighing scale, and the average results were determined. The harvest index was calculated by computing the ratio of grain yield divided by total biomass at the time of final harvest.
The calculation was performed using the formula shown below.
The sum of grain and straw yields was used to calculate biological yield.
Biological yield (g) = grain yield + straw yield was calculated using the formula biological
Determination of Leaf Cd Content
Following the washing process with deionized water, the leaf samples were subjected to drying in an oven at a temperature of 105ºC for a duration of 30 minutes. Subsequently, the samples were incubated at a temperature of 75ºC until a stable weight was achieved and maintained. The ground sample weighing 0.250 g was subjected to microwave digestion using a CEM MARS5 instrument (United States). The digestion process lasted for 30 minutes at a temperature of 180ºC, using 8 mL of HNO3. Afterward, the concentration of Cd in the leaves was quantified by ICP-MS (Agilent ICP-MS 7700ce, Agilent Technologies, Santa Clara, CA, United States).
Determination of Leaf Zn Content
Parts of the plant that were above ground, including the leaves, were taken from every treated plant and dried for three days in the sun and air. After that, they were dried in an oven at 60ºC for seventy-two hours and then crushed to pass via a 1 mm mesh. A cylindrical cup, holding 1 gram of the sample that had been dried in the oven, was put inside a muffle burner made of carbolite (AAF1100). The cup was heated to a temperature of 300ºC for a duration of one hour, resulting in the production of ash. The sample was cooled, and then the temperature was increased to 550ºC for 8 to 9 hours. After the addition of 2 milliliters of concentrated hydrochloric acid and an adequate amount of water, the sample was left to evaporate in the combustion chamber for a duration of 15 to 20 minutes on a heated surface. After cooling down again, ten milliliters of 20% hydrogen nitrate were added to the sample, which was then left in the water bath with the closed furnace lid for one hour. The sample was first thoroughly sanitized and filled up to a 100 mL capacity before it was filtered by using Whatman filter paper No. 2 into a volumetric flask. Subsequently, an ordinary solution was formed. In order to determine the amount of zinc present in the combination, an ICP-Optical Emission Spectrometer (Perkin Elmer, Optima 8300, produced by PerkinElmer Corporation in Norwalk, United States of America) was used.
Statistical Data Processing and Analysis
The present experiment was designed with three replications using the CRD statistical design. Statistix 8.1 software was used to perform a two-factor analysis of variance, and Tukey’s test was employed for comparing the means at the P≤0.05 level of significance. The Pearson correlation coefficient was determined using the statistical software Origin Pro 2022, and Microsoft Excel (Version Office 365) was used to construct the graphics of the obtained data.
Results
Morphological Parameters
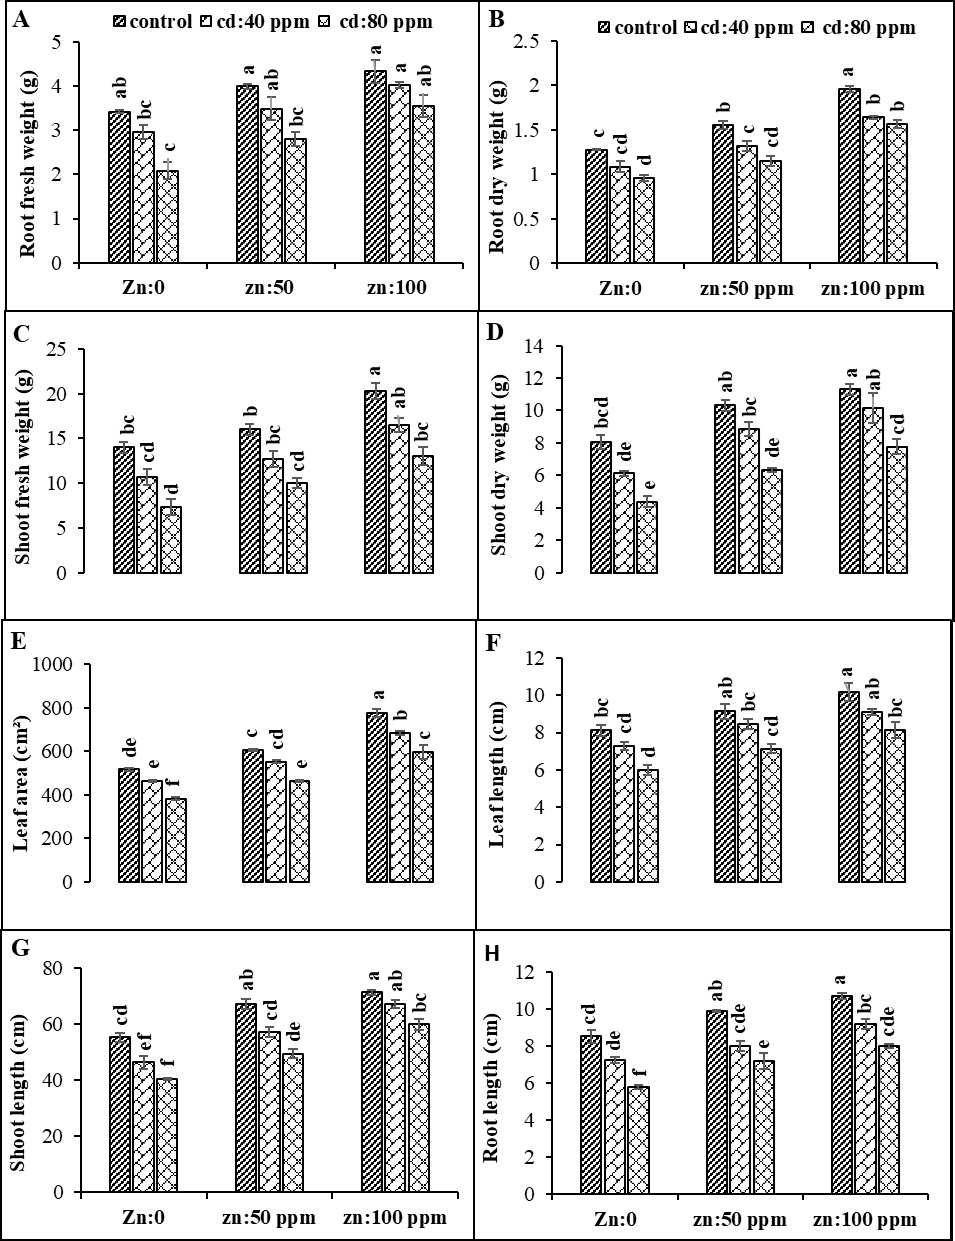
Statistical analysis revealed that a significant effect of Zn under cadmium stress for morphological attributes, i.e., shoot fresh weight, root fresh weight, shoot dry weight, root dry weight, root length, shoot length, leaf length, and leaf area. Cadmium stress causes significant reductions in all morphological attributes of sunflowers. The morphological attributes of sunflower were considerably affected by cadmium stress at 80 ppm level as compared to 40 ppm (Fig. 1). The most significant reduction of morphological features was observed at non-zinc treatments. Shoot fresh weight, shoot dry weight, and root fresh weight showed more reduction under Cd stress (47.6%, 45.68%, and 39.14%), respectively, in comparison with control (Fig. 1. C, D, A). Whereas root length, root dry weight, shoot length, leaf length, and leaf area showed less reductions (Fig. 1. H, B, G, F, and E) under Cd stress (32.03%, 25.9%, 27.03%, 26.5%, and 26.1%), respectively, in comparison with treatments. However, the application of Zn (100 ppm) played a crucial role in mitigating Cd stress, which significantly increases the shoot fresh weight, shoot dry weight, root fresh weight, root dry weight, shoot length, leaf length, root length, and leaf area up to (77.2%, 77.3%, 70.7%, 62.8%, 48.4%, 36.2%, 37.9%, and 56.2%), respectively (Fig. 1 and Table 1). However, the overall interaction between all factors Zinc×Cd was statistically non-significant.
Photosynthetic Pigments and Phenolic Compounds
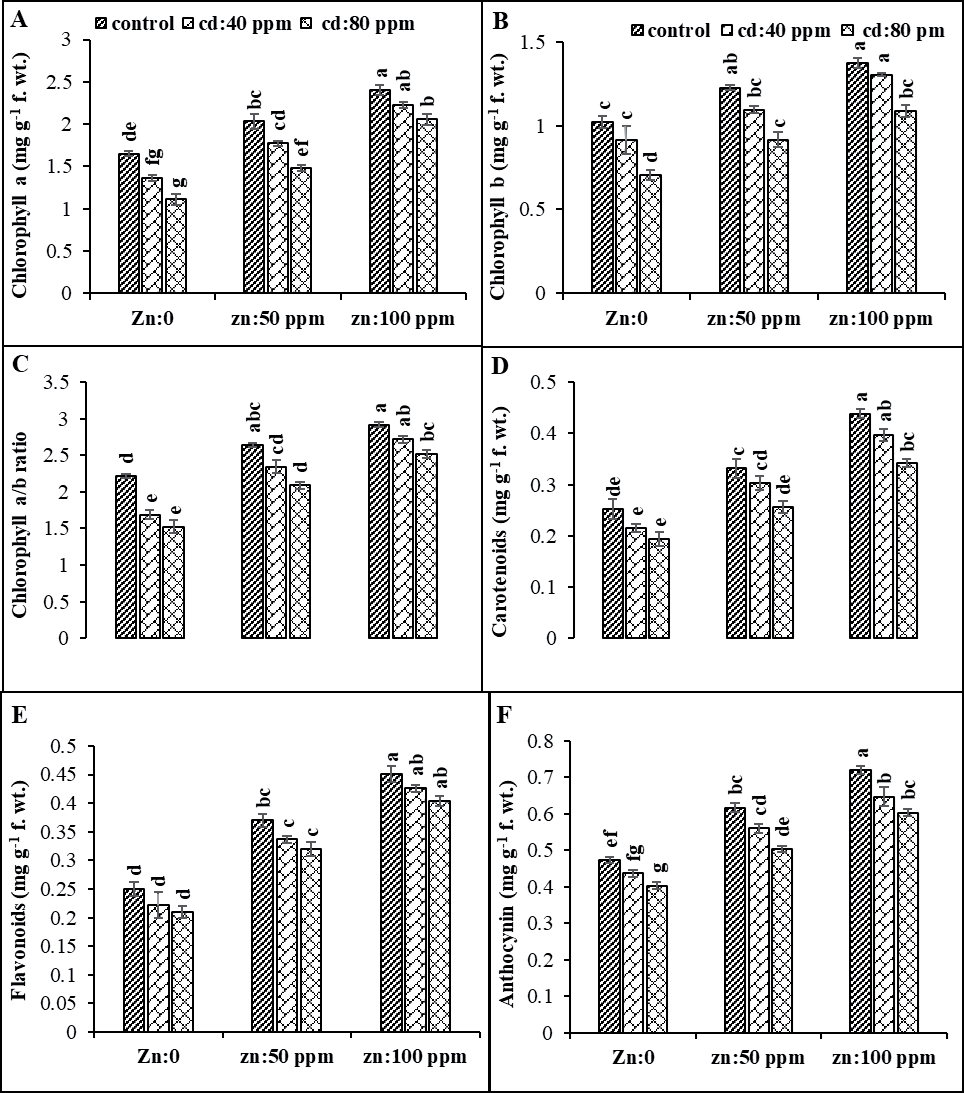
The acquired data for photosynthetic pigments showed a significant effect of Cd stress, which reduces the overall efficiency of the photosynthesis process. The higher level of Cd toxicity (80 ppm) reduced the Chl. a content (32.72%) (Fig. 2. A). Other photosynthetic pigments, e.g., Chl. b, Chl. ratio a to b, and carotenoids also showed maximum reduction under Cd stress up to 30.71%, 31.33%, and 23.15% as compared to non-stressed plants (Fig. 2. B, C, D). A significant effect of Zn application was recorded in the present study, which increased the Chl. a and carotenoids contents greatly by 85.28% and 84.88%, respectively. However, the application of Zn (100 ppm level as compared to 50) minimized the Cd-induced reduction. A significant increase of 53.82% and 65.64% was noticed for Chl. b and Chl. ratio a to b subsequently (Fig. 2). In short, there was no significant interaction seen between the stress caused by Cd and the administration of Zn. As the level of Cd toxicity increased from 40 ppm to 80 ppm, there was a reduction in photosynthetic pigments. Similarly, the higher level of Zn (100 ppm) application also enhanced the photosynthetic efficiency of sunflowers at the same rate (Table 1).
The data collected for flavonoids and anthocyanin showed that Cd stress significantly played a role in the overall reduction of plant phenolic contents. In the present study, flavonoids and anthocyanin contents were reduced by 16.37% and 18.37%, respectively, under the influence of Cd stress at an 80 ppm level (Fig. 2). However, the current investigation demonstrated considerable impacts of Cd toxicity on plants, which ultimately becomes the major constraint towards the self-defensive system of sunflowers against abiotic stresses. At the same time, application of Zn (100 ppm level as compared to 50) substantially increased the flavonoid contents up to 92.92% as compared to anthocyanin contents 52.11% in Cd-stressed plants (Fig. 2. E, F). The maximum increase in phenolic contents was recorded in non-stressed plants (Table 1). The interactive effect of Zn and Cd was noted to be non-significant.
Mineral Ions Content
The concentrations of various ions changed considerably under Cd toxicity. The Na+ ion concentration increased greatly in roots (61.02%) at 80 ppm Cd stress (Fig. 3. A), but the Na+ ion concentration in shoots was increased up to 29.42% under Cd stress (Fig. 3. B). However, the concentrations of root and shoot K+ and Ca2+ showed more reduction due to Cd stress. The root K+ revealed less reduction (35.72%) as compared to shoot K+ (43.87%) at 80 ppm Cd stress. The concentration of Ca2+ ions in roots showed more reduction (36.01%) as compared to shoot (26.98%) due to Cd stress at 80 ppm. Additionally, the exogenous application of Zn (100 ppm) showed significant results in terms of increased concentrations of root and shoot Na+, K+, and Ca2+ up to 22.25%, 91.12%, 103.92%, 45.72%, 68.07%, and 55.86%, respectively (Fig. 3. and Table 1). The combined effects of Zn and Cd were recorded as non-significant in the present study.
Yield Attributes
Cd stress and its interaction with plant yield attributes showed a significant trend at 40 and 80 ppm levels (Fig. 4). Recorded data for biological yield, harvesting index, number of seeds, 100-seed weight, oil contents, and protein contents revealed a decrease of 22.37%, 25.55%, 28.97%, 34.46%, 39.11%, and 42.84%, respectively, due to Cd stress at 80 ppm (Fig. 4. A-F). In the present study, the application of Zn as a growth promoter micronutrient for sunflowers showed maximum effects to mitigate Cd toxicity. With the application of Zn (100 ppm level), there was a substantial increase in yield parameters such as biological yield, harvesting index, number of seeds, 100-seed weight, oil contents, and protein contents up to 74.04%, 65.76%, 51.46%, 66.98%, 86.12%, and 104.37%, respectively (Fig. 4. A-F and Table 1). In conclusion, no significant interaction impact was seen between the stress caused by Cd and the administration of Zn.
Cd Contents in Leaf
The content of Cd in sunflower leaves exhibited considerable variations across several treatments of Cd-contaminated soil, e.g., 0 ppm, 40 ppm, and 80 ppm. At 0 ppm soil Cd control treatment, the Cd2+ concentration in leaves was maximum recorded up to 7 µg g-1 due to already present some Cd concentration in soil. With an increase in the concentration of soil Cd treatment, there was a significant rise in the Cd content in the leaves (Fig. 5. A).
Zn Contents in Leaf
Application of Zn at different levels, e.g., 50 ppm and 100 ppm, increased the Zn2+ concentration in leaves of sunflower plants under Cd toxicity, which improves the overall growth attributes of Cd-stressed plants. The maximum recorded concentration of Zn2+ in leaves of sunflower at 50 ppm and 100 ppm Zn application ranged from 21 to 32 mg/kg. At Zn control application, 5 mg/kg Zn2+ concentration was also recorded in leaves due to already present Zn in soil (Fig. 5. B).
Fig. 1.
Root fresh weight (A), Root dry weight (B), Shoot fresh weight (C), Shoot dry weight (D), Leaf area (E), Leaf length (F), Shoot length (G), Root length (H) of sunflower plant exogenously applied Zn with different levels as a growth promoter under Cd stress conditions. Significant differences among row spacing were measured by the least significant difference (LSD) at p>0.05 and indicated by different letters.
Correlation and Polar Heatmap Analysis
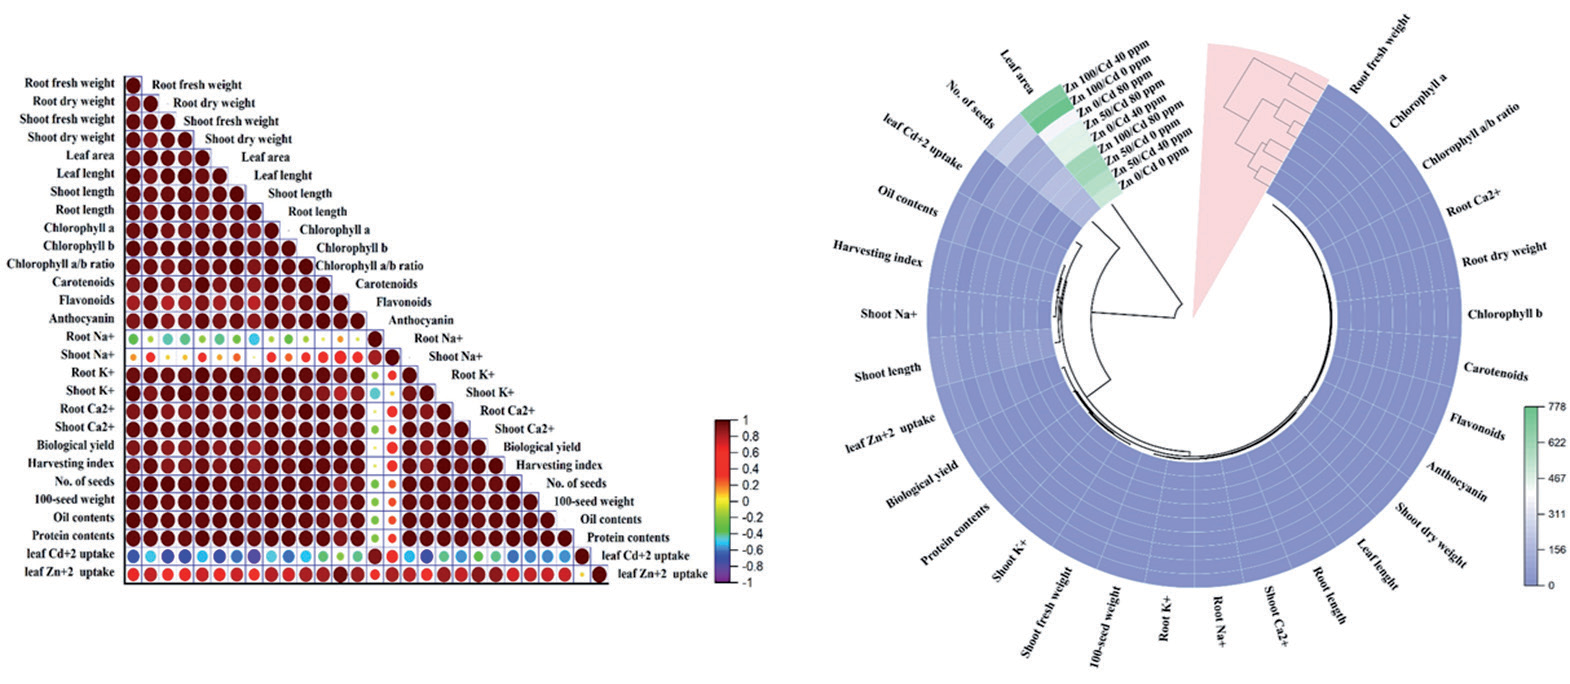
Pearson’s correlation study revealed a strong association between the morphological, photosynthetic, phenolic contents, mineral ions, and biological yield attributes of sunflowers. Various parameters, including root fresh weight, root dry weight, shoot fresh weight, shoot dry weight, shoot length, root length, leaf length, leaf area, anthocyanin, Chl. a, Chl. b, Chl. ratio a to b, and carotenoids, showed a strong positive correlation with the majority of indicators (Fig. 6). On the other hand, root Na+, shoot Na+, leaf Cd+2 uptake, and leaf Zn+2 uptake revealed a negative correlation with most indices. Shoot K+, root K+, shoot Ca+2, root Ca+2, flavonoids, biological yield, harvesting index, number of seeds, 100-seed weight, oil contents, and protein contents did not show considerable correlations with most indexes (Fig. 6).
The results for all assessed characteristics of sunflowers in the nine treatments were shown in a polar heat map along with a dendrogram, facilitating basic comparisons of the effects of the treatments on the desired plant attributes. The findings revealed that nine therapies may be categorized into four main categories. Zn 50/Cd 80 ppm and Zn 0/Cd 80 ppm are clustered together; Zn 100/Cd 80 ppm, Zn 50/Cd 40 ppm, and Zn 0/Cd 40 ppm are clustered together; Zn 100/Cd 40 ppm, Zn 100/Cd 0 ppm are clustered together; and Zn 50/Cd 0 ppm and Zn 0/Cd 0 ppm are clustered together. Polar heatmap with dendrogram overall indicating high measured values for leaf area, medium measured values for number of seeds, and low measured values for all other growth, photosynthetic, phenolic contents, mineral ions uptake, and biological yield attributes of sunflower (Fig. 6).
Fig. 2.
Chlo. a (A), Chlo. b (B), Chlo. a/b (C), carotenoids (D), flavonoids (E), anthocyanin (F) of sunflower plant exogenously applied Zn with different levels as a growth promoter under Cd stress conditions. Significant differences among row spacing were measured by the least significant difference (LSD) at p>0.05 and indicated by different letters.
Discussion
Plant growth is restricted, and plant production is negatively impacted by abiotic factors such as heat, salt, drought, and heavy metal stress, particularly cadmium [21]. The results of this experiment confirm our hypothesis that the use of Zn substantially ameliorates the morphological, photosynthetic, and yield attributes along with the phenolic and mineral ion contents of sunflowers under cadmium stress. Due to the negative effects of Cd strain, SFW, SDW, SL, RFW, RDW, RL, LA, and LL significantly decreased in contrast to the control treatments (Fig. 1). These drops in morphological attributes of sunflower were due to the harmful and toxic effects of Cd stress because Cd causes oxidative and ultrastructures damages, nutrient imbalance, and localization inside the subcellular space of plants [22]. In the current investigation, the application of Zn (100 ppm as compared to 50 ppm) shows a substantial function in mitigating Cd stress. The positive role of exogenous application of Zn was also previously studied by Rizwan [23]. The ameliorated proliferation of plants in terms of morphological attributes like SFW (77.2%), SDW (77.3%), SL (48.4%), RFW (70.7%), RDW (62.8%), RL (37.9%), leaf area (56.2%), and leaf length (36.2%), respectively, were due to the application of Zn because it promotes cell division and elongation [24]. Auxin biosynthesis is improved with the usage of zinc, which is one of the insights given for the increases in plant dry and fresh weights [25]. In terms of the degradation of physiological and biochemical processes, excessive levels of cadmium stress (80 ppm as compared to 40 ppm) have a detrimental impact on the reduction of plant development, which ultimately causes damage to the defensive system of the plant. Plants can produce phenolic substances as a defensive strategy in order to mitigate the detrimental effects that metal stress puts on the surface of the cell which can lead to oxidative damages such as membrane damage and cell death [26]. In the present trial, Cd stress triggered a significant reduction in polyphenolic compounds of plants such as flavonoids and anthocyanin up to 16.37% and 18.37%. As a consequence of this, plants become more vulnerable to the harm that is brought about by abiotic stressors. However, the application of zinc played an antagonistic role against Cd stress and improved the plant polyphenolic compounds, e.g., flavonoids (92.92%) and anthocyanin (52.11%). Plants are protected from oxidative stress by the synthesis of polyphenolic chemicals, which have the ability to reduce the generation of free radicals and may function as antioxidants for metal ions [27].
Fig. 3.
Root Na+ (A), Shoot Na+ (B), Root K+ (C), Shoot K+ (D), Root Ca2+ (E), Shoot Ca2+ (F) of sunflower plant exogenously applied Zn with different levels as a growth promoter under Cd stress conditions. Significant differences among row spacing were measured by the least significant difference (LSD) at p>0.05 and indicated by different letters.
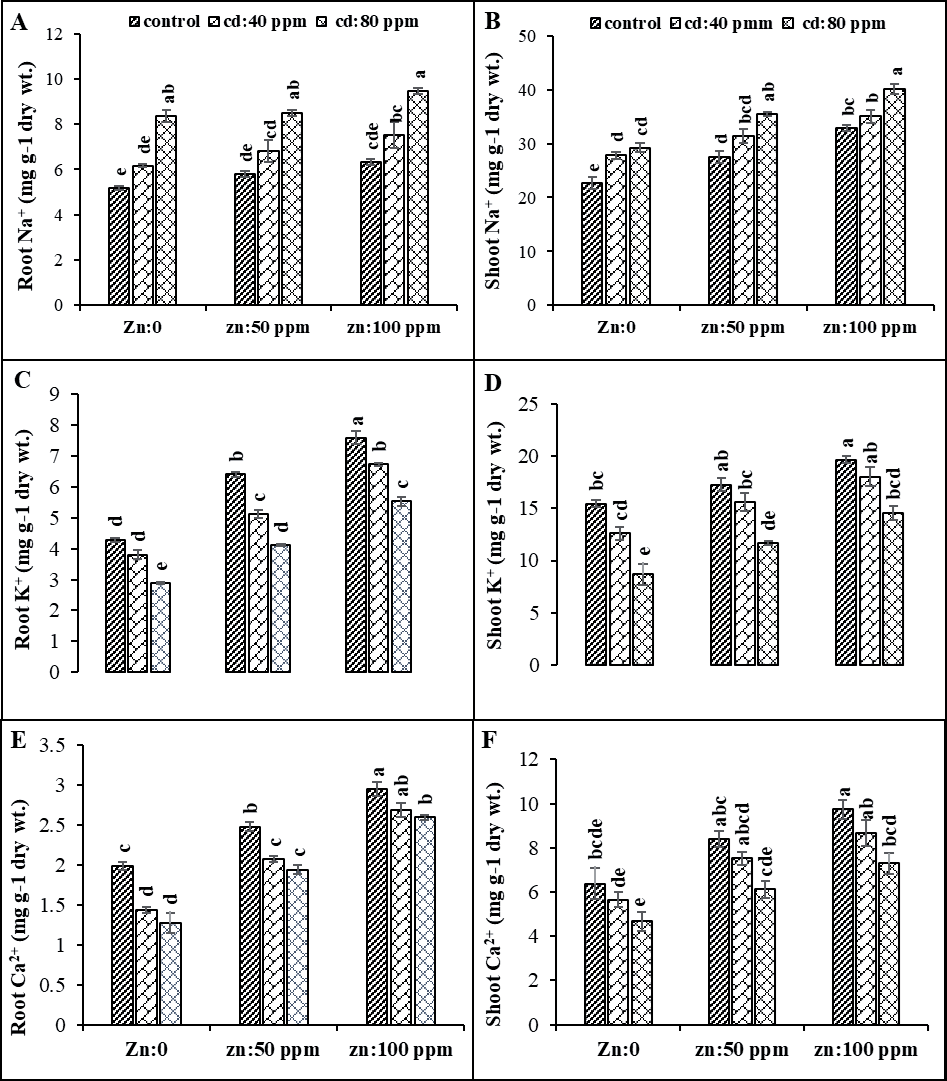
Fig. 4.
Biological yield (A), Harvesting index (B), Number of seeds (C), 100-seeds weight (D), Oil contents (E), Protein contents (F) of sunflower plant exogenously applied Zn with different levels as a growth promoter under Cd stress conditions. Significant differences among row spacing were measured by the least significant difference (LSD) at p>0.05 and indicated by different letters.
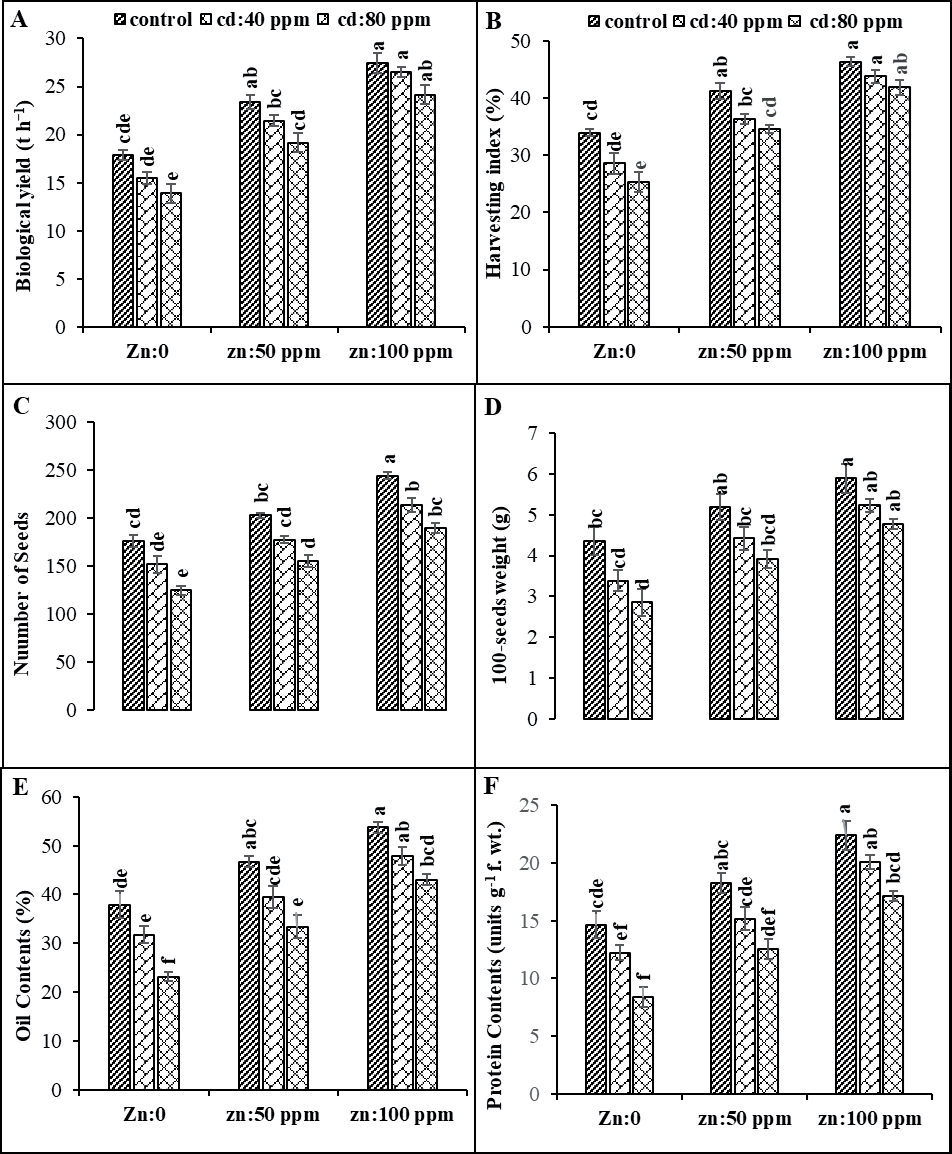
Table 1.
Mean values of morpho-physiological, biochemical, and biological yield attributes of sunflower under cadmium stress.
The outcomes of the experiment that was being conducted revealed that yield attributes of sunflowers, such as biological yield, harvesting index, no. of seeds, 100-seed weight, oil contents, and protein contents, were decreased up to 22.37%, 25.55%, 28.97%, 34.46%, 39.11%, and 42.84%, respectively, due to the application of 80 ppm Cd stress. Marques [28] also illustrated that cadmium contamination has greatly reduced the accumulation of biomass in sunflower plants. Exposure to cadmium leads to the suppression of plant development due to its harmful effects, which also affect the regulatory functions of important metabolic enzymes and stimulate leaf necrosis [29]. As a result, the yield of overall plants is reduced considerably. However, the application of zinc in plants has been proven effective in enhanced accumulation of their dry matter and protein contents as well as their total agricultural yield since it is essential for the formation of proteins and the breakdown of carbohydrates [30]. In our research trial, results revealed that exogenous applied Zn (100 ppm) significantly enhanced the yield attributes, e.g., biological yield (74.04%), harvesting index (65.76%), no. of seeds (51.46%), 100-seed weight (66.98%), oil contents (86.12%), and protein contents (104.37%) of sunflowers. The chlorophyll concentration, e.g., Chl. a (32.72%), Chl. b (30.71%), Chl. ratio a to b (31.33%), and carotenoids (23.15%), significantly reduced due to the toxic effects of Cd in contrast to control treatments. A decrease in the content of photosynthetic pigments has been observed as a frequent indication of toxicity to metals in several plant species [31]. Haseeb and Maqbool [32] studied that reduction in light-absorbing components of photosynthesis machinery (Chlorophyll a, b, ratio a to b, and carotenoids) was observed in sunflower plants due to noxious effects of abiotic stresses. According to studies by Vijayaragavan [33] and Touiserkani and Haddad [34], cadmium decreased the concentration of chlorophyll by either causing the Mg ion to be removed from its binding site in chlorophyll (which led to the deterioration of the chlorophyll molecule) or by hindering the activity of enzymes involved in the production of chlorophyll, such as protochlorophyllide reductase, porphobilinogen deaminase, and aminolevulinic dehydratase, which led to a shortage of Fe2+ and Mg2+, which in turn caused carbonic anhydrase activity to be inhibited due to Zn2+ limited supply [35]. However, in the present trial application of zinc enhanced the photosynthetic capacity of sunflowers up to 85.28%, 53.82%, 65.64%, and 84.88% were noticed for Chl. a, Chl. b, Chl. ratio a to b, and carotenoids subsequently under Cd stress. Wu [36] demonstrated that the use of Zn’s impact on photosynthesis’s enzyme activity might be the cause of improving photosynthetic attributes, as foliar treatments may enhance the associated zinc enzyme [37]. Previous studies have shown that the combination of amino acids and microelements enhances the rate of photosynthesis in plants when applied independently or in response to external environmental stressors [38, 39]. Research has also shown that the reduced toxicity of Cd in wheat plants or the enhanced presence of zinc as a plant microelement might be a significant factor contributing to the increase in photosynthetic indices. The concentration of Na+ increased in both shoot and root while the concentrations of Ca2+ and K+ decreased due to Cd stress. Kosakivska [40] explained that Cd inhibits nitrate reductase, reducing the transport and intake of nitrate and interfering with the absorption of Ca, P, K, Mg, and water. Metal transporters enable the transportation of inorganic minerals to and from vascular bundles during the loading and unloading process. Increased levels of Cd will lead to detrimental effects due to the interactions between Cd ions and other elements. Hence, the translocation of Cd ions in plant cells would be diminished if they were conveyed by cation channels or other transporters [41]. Nevertheless, in the current study, the use of zinc substantially increased the levels of plant root and shoot Na+, K+, and Ca2+ up to 22.25%, 91.12%, 103.92%, 45.72%, 68.07%, and 55.86%, respectively [42]. The decrease in the accumulation of mineral ions has an adverse effect on the processes of metabolism and photosynthetic indices [43]. A key approach to detoxifying heavy metal-contaminated soils is called phytoextraction, which functions via the use of accumulators to draw toxins from the soil and transfer them into plants. A phytoextraction plant species with excellent metal resistance and biological accumulation index should be ideal for the reclamation of heavy metal-affected soils for sustainable agriculture [44]. In our current research trial, there was considerable Cd2+ accretion in the leaves of sunflower plants, and Cd concentration in the leaves showed a substantial elevation with the increasing levels of Cd soil treatments, e.g., 40 ppm and 80 ppm (Fig. 5. A). At higher levels of Cd soil treatment, various attributes (photosynthetic, growth, and yield attributes) of sunflowers were affected considerably in terms of lower photosynthetic efficiency and reduced biological yield due to Cd toxicity. Lux [45] studied that the majority of plants are hazardous to leaf Cd contents over 5-10 μg g−1. In the present study, the application of Zn significantly reduced the Cd-induced losses in sunflower plants. Zinc (Zn) is a crucial micronutrient that serves as a constituent of several enzymes responsible for regulating multiple metabolic events in plants. It is also necessary for the creation of auxins and proteins. Additionally, it facilitates enhanced assimilation of nitrogen (N) and phosphorus (P) by plants [46]. As the concentration of Zn application increases from 0 ppm (control) to 100 ppm, the Zn2+ concentration in the leaves of sunflower also increases, ranging from 5 to 32 mg/kg. This indicates the considerable effect of Zn application to improve the growth, photosynthetic, mineral ion uptake, and yield attributes of sunflower plants under Cd-stressed conditions.
Fig. 5.
Cd+2 uptake in leaf (A), Zn+2 uptake in leaf (B) of sunflower plant exogenously applied Zn with different levels as a growth promoter and Cd+2 as an abiotic stress also applied with different levels. Zn+2 and Cd+2 uptake increases as their level of application increases. Significant differences among row spacing were measured by the least significant difference (LSD) at p>0.05 and indicated by different letters.
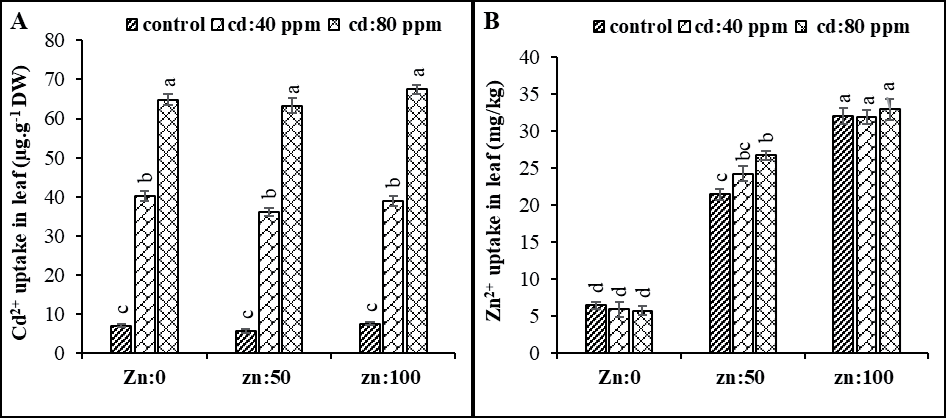
Fig. 6.
Pearson’s correlation matrixes constructed (On Left Side) for morphological, photosynthetic, phenolic contents, mineral ions uptake, and biological yield attributes of sunflower under Cd stress. *Significant at p≤0.05%; **Significant at p≤0.01%; ***Significant at p≤0.001%. Polar heatmap analysis between various attributes of sunflower (On Right Side) showed the impact of Zn application under Cd stress on morphological, photosynthetic, phenolic contents, mineral ions uptake, and biological yield attributes of sunflower; Zn:0/ Cd:0, Zn:50 ppm/ Cd:0, Zn:100 ppm/ Cd:0; Zn:0/ Cd:40 ppm, Zn:50/ Cd:40 ppm, Zn:100/ Cd:40 ppm; Zn:0/ Cd:80 ppm, Zn:50/ Cd:80 ppm, Zn:100/ Cd:80 ppm.
Conclusions
The present study indicates the alterations in sunflower plants exposed to Cd stress in combination with Zn usage. The usage of Zn in general agricultural practices overall ameliorates the harmful effects of Cd toxicity that pose harmful impacts on morphological, photosynthetic, phenolic contents, mineral ions, and biological yield attributes of plants. It was also studied that Cd toxicity causes oxidative and ultrastructure damage, nutrient imbalance, and subcellular localization in plants that ultimately impair plant development and adversely affect plant productivity. Translocation and uptake of mineral ions by plants also become disturbed due to Cd stress. However, application of Zn distinctly revealed its beneficial contribution to recouping losses carried on by stress. Furthermore, experiments needed to be accomplished alongside other micronutrients to investigate hazardous metal phytoremediation procedures in field trials on a larger scale.

