

Introduction
Due to ongoing climate change, data on plant diversity and distribution are essential for conservation biology and resource management at all scales and must be continuously gathered. Climate change has significantly altered the distribution and abundance of species over the last three decades and has been linked to one extinction at the species level [1]. The Arabian Peninsula has a wide climatic spectrum, ranging from the Asir Province’s snows to the Arabian Gulf’s oppressive humidity [2]. Even though several places have been carefully examined for the effects of climate change on floristic composition [3]. Saudi Arabia’s scientific knowledge and literature on climate and climate change are fragmented, scattered, and inadequate [4] investigated how general circulation models predicted the effects of rising temperatures and climate change and decreasing precipitation on Saudi Arabia’s agriculture and water resources. The Kingdom of Saudi Arabia (KSA) is one of the most vulnerable nations to climate change because of its continental climate, which has harsh winters, scorching summers, and low rainfall [2]. Recently, [5] issued a warning to those interested in wild plants and to governments to take appropriate measures to protect the arid environment threatened by the impact of climate change.
A significant threat to climate change is posed by invasive plants, and greater global connectivity has greatly increased the variety and scope of such invasions [6]. Semi-arid areas have already been overrun by invasive plants, which deplete soil nutrients and destroy natural habitats [7]. There is a dearth of research on how invasive species affect the ecology in western Saudi Arabia. Nevertheless, it is regarded as one of the most crucial factors when developing strategies for the conservation of biodiversity [8]. There are 55 exotic or extraterrestrial species in Saudi Arabia, most of which are restricted to populations of no more than 2% in the areas where they are found, but predictions indicate that they may eventually spread to populations of more than 10% or 15% within the next few years [9]. In another research, 42 alien plant species from 15 families and 11 different Saudi governorates were identified [10]. The genus Prosopis, which includes forty-four species native to North, South, and Central America, as well as the Caribbean, is one of the groups of invasive taxa [11] and is regarded as the most dangerous invasive trait [12-14]. It also slowly replaces native species, changes ecological processes, and has a big effect on the area’s biodiversity [5, 15, 16]. Previous studies [17] recorded that its allelochemicals increase the species’ dominance in interspecific competition in the invaded environment. The plant’s roots, flowers, leaves, and fruits all generate these compounds [17]. These allelochemicals are thought to be the cause of the plant’s invasiveness P. Juliflora can survive in a variety of soil types and climatic conditions, it spreads quickly and takes over many habitats [18-20]. The coppice development of P. juliflora does not appear to be impacted by any known growth-inhibiting soil characteristics, such as excessive alkalinity, salt, low fertility, high soil temperature (up to 70ºC), or heavy rainfall (up to 5000 mm), which are regarded to restrict plant growth [6, 7]. Additionally, the broad, thick crown of P. juliflora inhibits the development of understory shrubs and vegetation. Furthermore, the mode of seed dissemination of P. juliflora is great for delivering good, nourishing fruit to birds and animals, which speeds the spread to remote locations [5]. The western region of Saudi Arabia, with its diverse habitats, is considered among the richest regions of biodiversity in the Arabian Peninsula with the presence of a large number of endemic, rare, threatened, and endangered plant species [21-24].
Finding management answers to pressing environmental issues such as climate change and the spread of invasive species is the focus of a large community of ecologists and biodiversity enthusiasts [25]. Among many other options, the use of tracking technologies that can detect environmental changes quickly and over time has emerged as one of the most popular approaches. This ecological observation allows for more informed and effective management options [26]. We anticipate that P. juliflora invasion and expansion will lead to localized extinctions of the local flora, resulting in a decline in species richness and variety. The current study has two goals. The first is to find out how P. juliflora affects the native plants in the Jeddah area. The second is to find out how this species affects the soil’s physical and chemical properties.
Material and methods
Study area
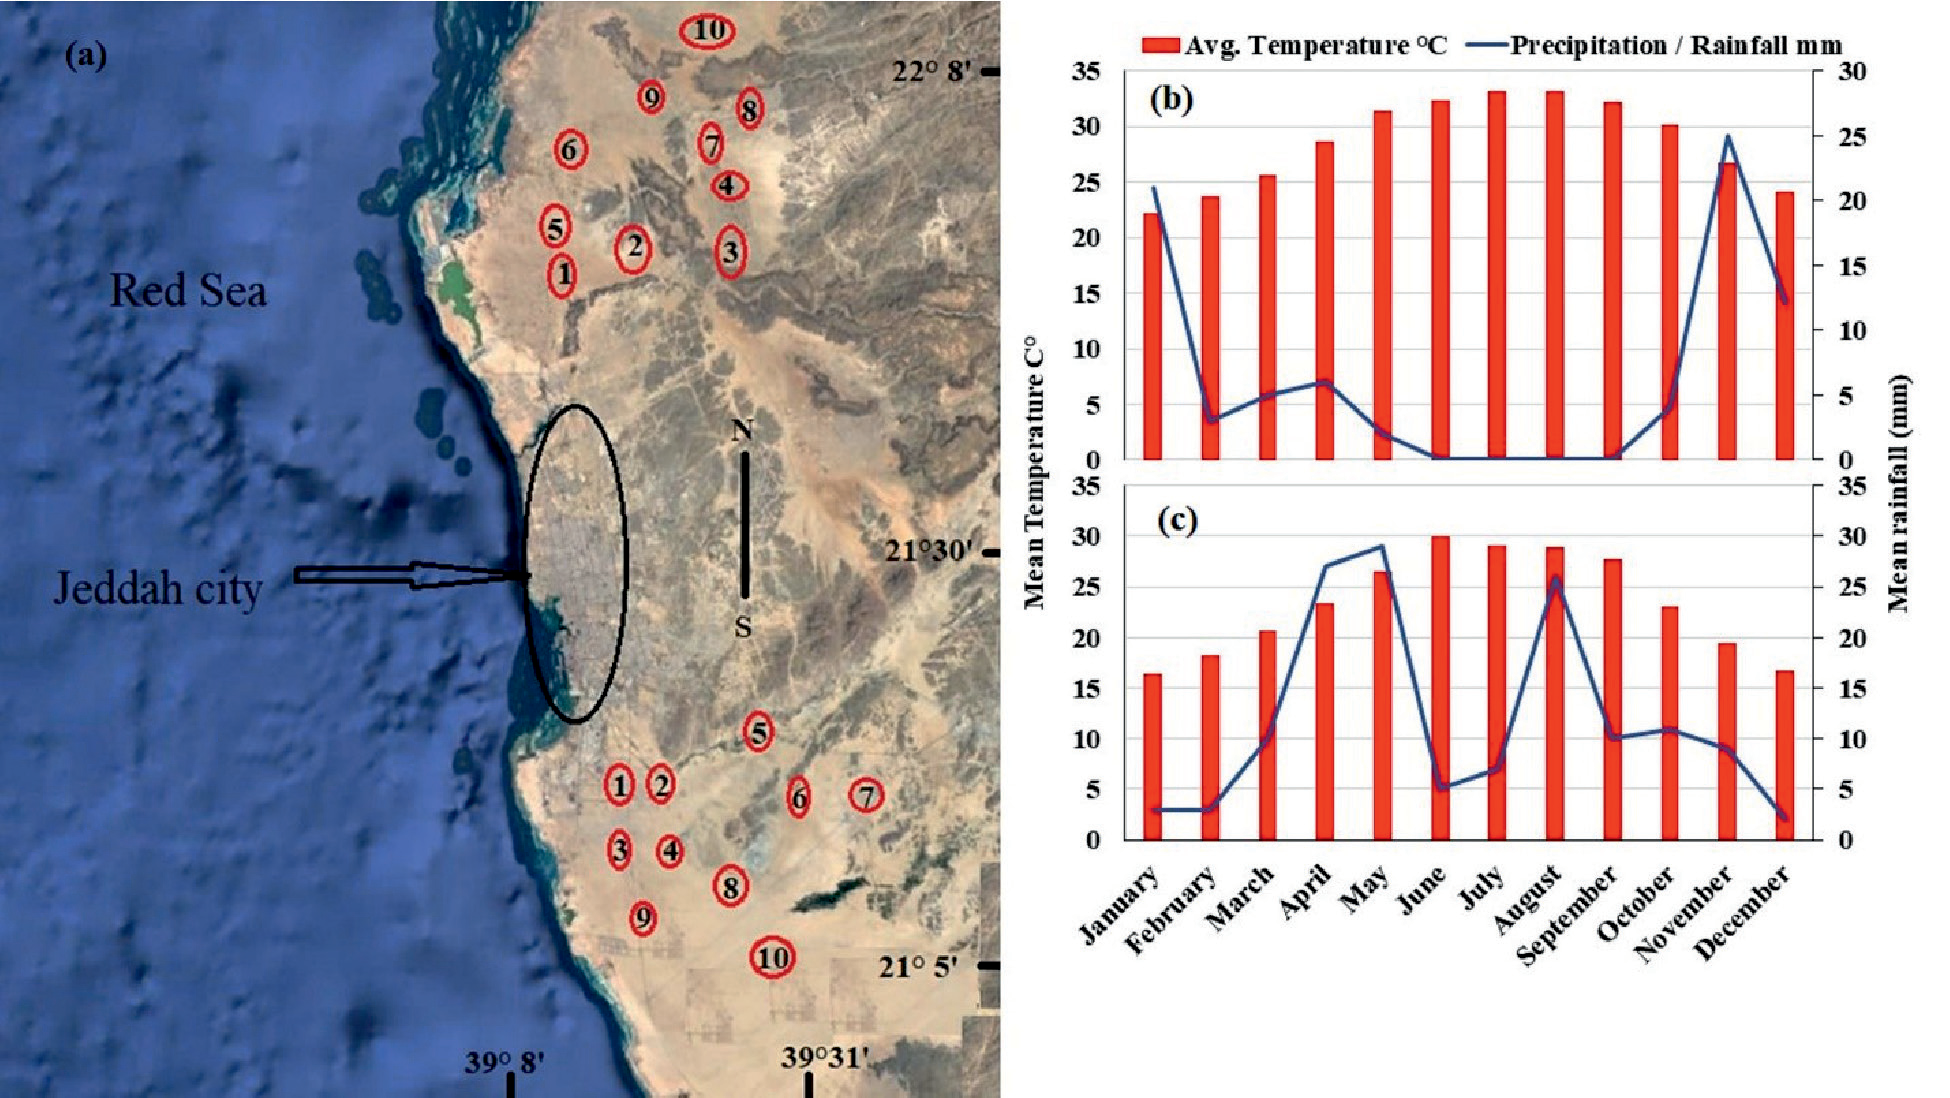
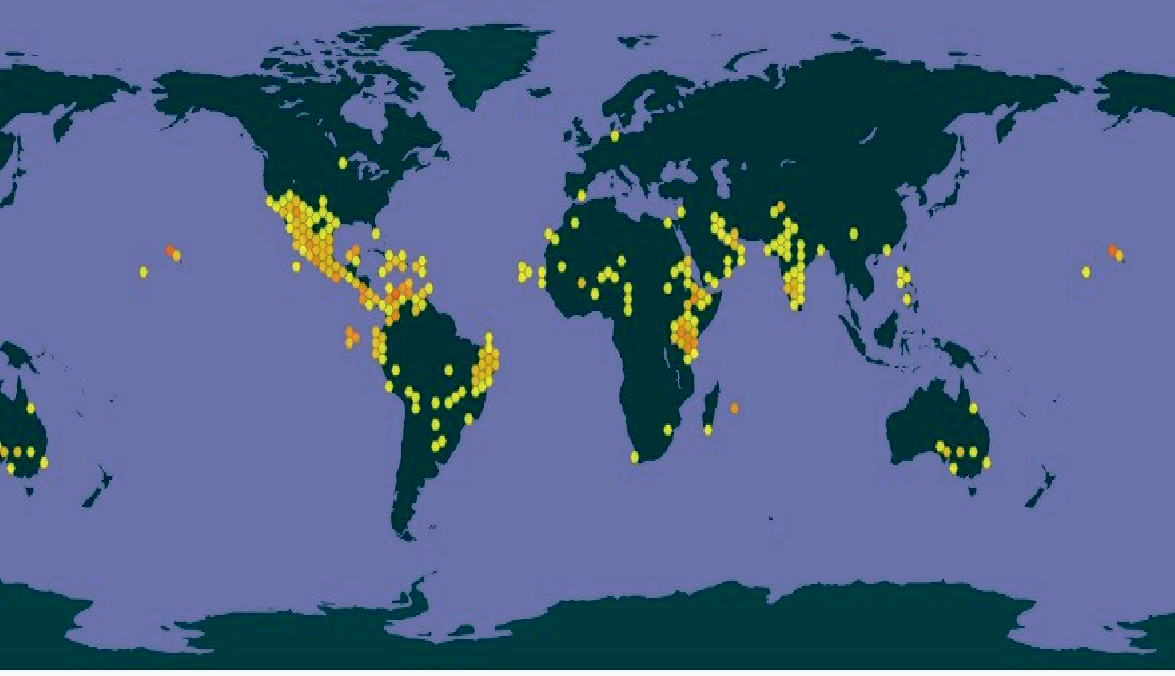
The studied area is Jeddah City, located in Saudi Arabia between 21.4858°N and 39.1925°E Fig. 1a). The climate is characterized by warm winters and high summer temperatures. The region experiences arid weather; the average annual rainfall is 35.1 mm. In addition to being sparse, the rainfall is erratic and varied, ranging from 0 to 70 mm. In the past two years, there have been intermittent, torrential downpours on one or two days. The monthly high for air temperature is 37.4ºC in June, and the monthly low is 13.2ºC in January. (Fig. 1b). Also, we obtained the presented data of the global distribution of P. juliflora from the Global Biodiversity Information Facility [27] (Fig. 2).
Measurement of Aridity indices of the Study Area
The climatic data for the period (1970-2021) was obtained from Google Earth Engine [28]. Via registration for (New Script - Earth Engine Code Editor (google.com), then Browsing for https://earthengine. google.com/ and Choosing (Datasets) then (Modis). A simple technique to visualize the ratio of precipitation to evaporation is using aridity indices. The climate change in the Jeddah area was estimated by calculating three different aridity indices as follow: the Lang index, the Emberger aridity index, and the Martonne index.
Fig. 1.
A location map shows the studied stand locations a), average temperatures, and rainfall for North b) and South c) Jeddah.
Lang index [29] was calculated as described in the following Equation (1):
where L stands for Lang’s rainfall factor, R stands for average rainfall, and T stands for average temperature.
Emberger aridity [30] was calculated as described in the following Equation (2):
where Ip is the Emberger index, p is the average annual precipitation, T is the average maximum temperature for the hottest month, while t is the average lowest temperature for the coldest month.
De Martonne index [31] calculated as described in the following Equation (3):
where IDM = De Martonne’s index, Pav. = average rainfall, Tav. = average temperature.
Impact of P. juliflora on Native Plant Species
The study area was divided into two main locations, south and north Jeddah; twenty sites were randomly selected from both locations, ten locations in each south and north of Jeddah. Forty stands were randomly distributed in both south and north Jeddah, with each stand selected to have a reasonable level of physiognomic homogeneity and to be as like one another as feasible (the same habitats and the same tree age). These stands, each measuring 104 m2 (100 m × 100 m), covered the density variations in the chosen sites. In each stand, ten quadrats (100 m2) were distributed over five transects: five beneath and five outside of the P. juliflora canopy. A species list was recorded for each stand. A calculation was made to determine the species’ absolute density (individuals of a certain species rooted within one hundred m2). Samples were gathered from January to April, just before the annuals disappeared, due to the hot climate in the study area. The environmental affairs agency and wildlife authority of the Jeddah Governorate’s regulations and laws were followed when collecting the plant samples. All plant species were identified by Dr. Mohammed A. Fadl, an associate professor of plant taxonomy, and his findings were corroborated by published research [32, 33] and herbaria voucher specimens. The International Plant Names Index was used to verify the species list’s nomenclature (www.ipni.org.). The gathered samples were stored in the biology department’s herbarium at the Taif University. According to Raunkiaer [34] the life forms of each species were determined. Relative density (RD) is a measure of a species’ overall number of individuals in proportion to all other species’ individuals, determined as:
The biogeographic affinities of the investigated species were determined at each elevation belt according to [35, 36].
Soil sampling and analyses
To reveal the effect of P. juliflora on soil traits, four soil samples (from zero to 30 cm) were collected under and outside a P. juliflora tree in both North and South Jeddah. The four samples from each location were chosen randomly under and outside four different trees. These four soil samples were carefully blended to form a composite sample, which was then air-dried. Air dried soil samples were crushed, homogenized, and sieved through a 2 mm sieve to remove large particles. The amount of organic matter in the 2 mm soil fraction was calculated using the mass lost by combustion at 430ºC. Conductivity and pH meters were used to measure the electrical conductivity (EC) and pH of soil water extracts (1:2.5 soil: water). Utilizing 2 M KCl, the available nitrogen was extracted using the micro-Kjeldahl technique. To determine the amount of accessible phosphorus, Olsen’s solution (sodium bicarbonate) was employed as an extracting agent. Na and K were calculated using flame photometry [37]. The total phenolics content of each solution was determined by measuring the spectrophotometric absorbance at 700 nm and using ferulic acid as a standard [38]. Three replicates for each estimation were kept.
Results
Habitats in which P. juliflora Has Been Recorded
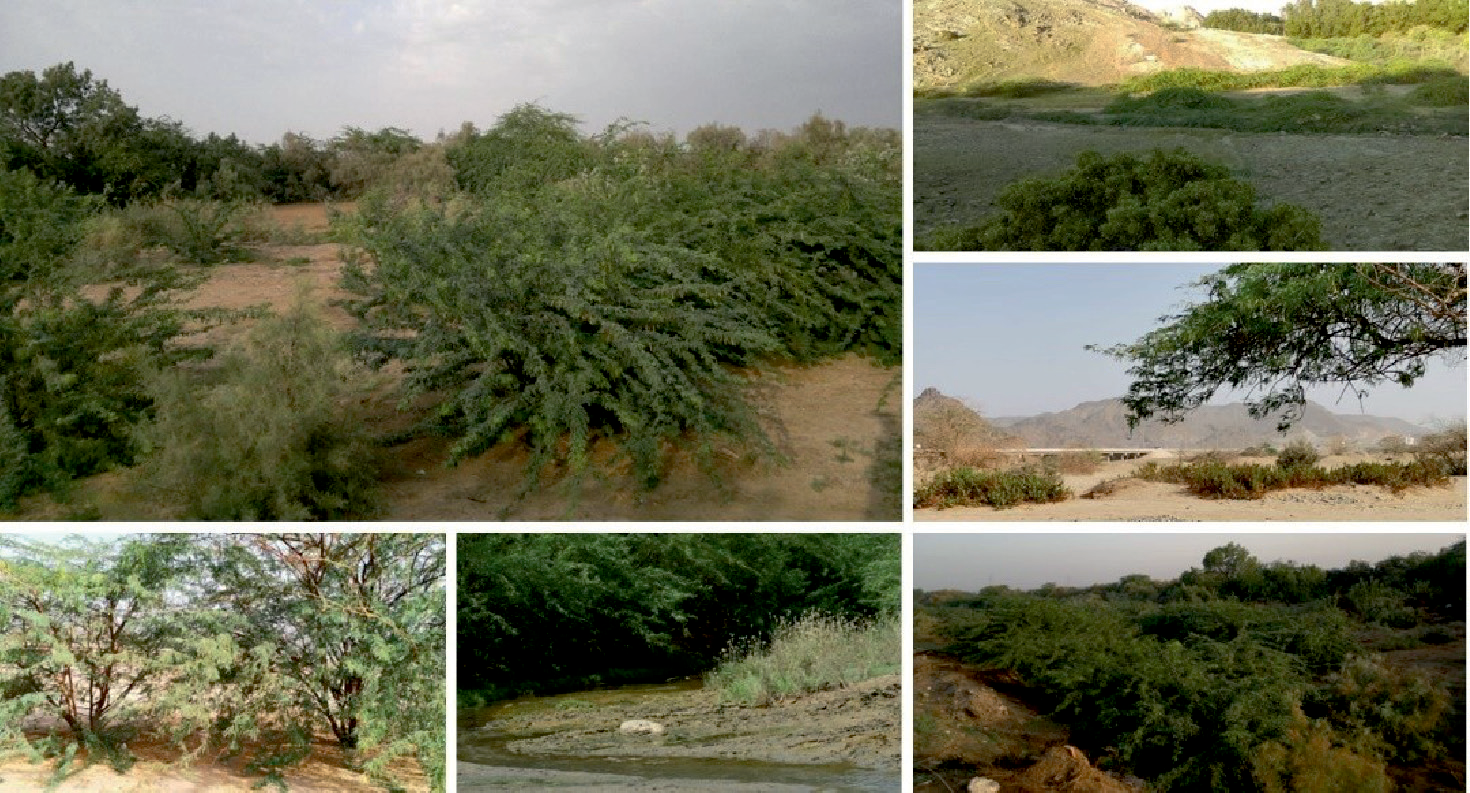
P. juliflora was recorded in a broad range of habitats, including swampy habitats, sand dunes, and inland wadis (Fig. 3). It was observed in the most hostile land unfit for any other plant species, and it is usually found in places where salinity, soil fertility and water are the primary limiting variables for plant growth. During the research, it was observed that the plant spreads swiftly in fine and medium sand soils, but not in compacted soils. In addition, P. juliflora was recorded in rocky habitats exposed to erosion factors where its rocks were shattered and quantities of fine sand were transported to it by the wind to be soft sandy soil, constituting a soil not more than one meter deep, while the plant was not found in rocky areas, resistant to erosion. In the present study, we have noticed that P. juliflora invaded the habitats of economically and medically important plants like Salvadora persica and Rhazya stricta in North Jeddah, as well as the Acacia ehrenbergiana community.
Aridity Indices of the Study Area
The aridity indices for the study area show that the area is very dry, with no more than 2.15, 27.8 and 10.17 for the Lange index, Emberger index, and De Martonne index, respectively (Fig. 4). By comparing the aridity indices for the years 1970 and 2021, it was noted that the three indices decreased by 36, 33.5 and 0.5% for the Lange index, Emberger index, and De Martonne index, respectively.
Effects of P. juliflora on Soil Characters
Table (1) shows that the pH of all the two locations decreased by 6.5%, in contrast the levels of Na, K, N, EC, and organic matter rose under the P. juliflora trees rather than outside. The rise in sodium content varied from 25.5 to 108%, whereas the increase in organic matter was 33 to 160%. While the phosphorus content of the soil (under the tree) increased by 44% to 66% compared to the concentration outside the tree. Soil salinity (EC), potassium, and nitrogen content increased under the tree by 27 to 124, 31 to 45, and 46 to 68%, respectively, compared to their contents outside the tree (Table 1). P. juliflora significantly increased the soil’s phenolic content by 200% and 160% in north and south Jeddah, respectively.
Effect of P. juliflora on the Associated Native Species
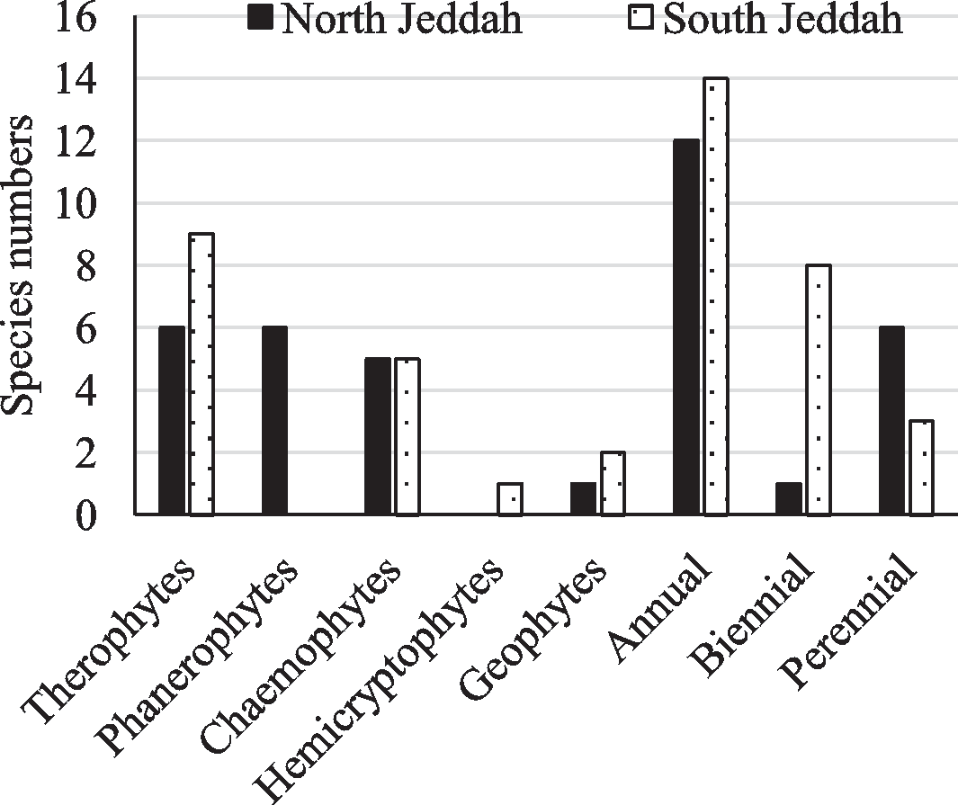
In the North Jeddah region, twenty-nine species belong twenty families were recorded, where P. juliflora is found (Table 2). More than 63% of the associated native species disappeared under P. juliflora tree, while the density of the rest was reduced by a range between 54 and 97%. The associated species number recorded in the South Jeddah area, where P. juliflora is found was thirty species (Table 3). More than 65% of the plant species disappeared under P. juliflora, while the density of the rest was reduced by a range between 58 and 95%. Results showed that the majority of the disappeared species were annuals in their habit and therophytes (life forms).
Life Forms and Habits of the Disappeared Species
Fig. 5 shows that the annuals species recorded the largest percentage of plants that disappeared due to the P. juliflora tree, it exhibited 82% in the South Jeddah area, 66% in the North Jeddah area. Therophyts had the largest share of the species that disappeared from under the P. juliflora tree in the four sites that were studied, the largest percentage was recorded in South Jeddah (82%). Phanerophytes, also exhibited a higher percentage of the disappeared species in North Jeddah area, while hemicryptophtes showed a high percentage in South Jeddah areas.
Discussion
Distribution of P. Juliflora
In the current study, P. juliflora has been recorded in many different soil types and habitats, such as sand dunes, coastal flats, and broken clays, particularly where water, soil fertility, and salt are the main things that stop plants from growing. In addition, it was observed that the plant can survive and even flourish on some of the harshest terrain unsuitable for the majority of native species. Previous observation could be attributed to the wide ecological range of P. juliflora. [2] highlighted its tolerance the harsh environmental conditions such as aridity, high temperature salinity and water flooding, that indicate its ability to thrive in arid, or seasonally dry, environments. Furthermore, its deep taproot, P. juliflora can also thrive next to canals, irrigation ditches, lakes, and other bodies of water. It can grow well along the coast where the water is salty, on beaches, in salt flats, and even near mangroves in Sri Lanka [12].
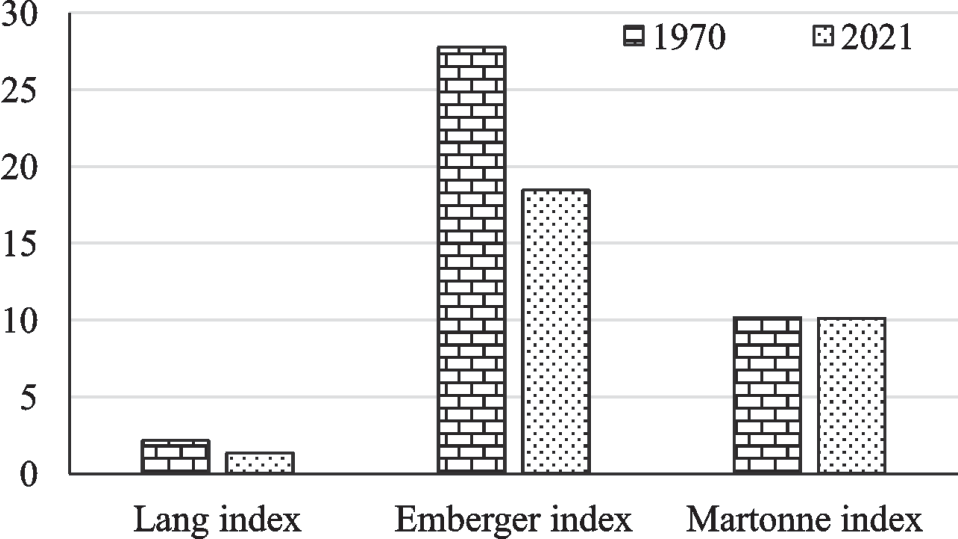
Table 1.
Effect of P. juliflora canopy on some chemical characters of soils under and outside the canopy. The data are mean values with standard deviations (n = 4). Different letters (in the same row) indicate a statistically significant difference in means for the same soil parameter for one location, at least at the 0.05 significance level.
It was reported that the exponential growth rate of 4-15% per year of the Prosopis tree has a negative effect on ecosystem functions and the way people make a living [14].
In was recorded in a previous study [12] that P. juliflora seedlings have the capacity to develop tap roots that extend beyond three meters into the soil and grow actively with expanding lateral surface roots for several months of the rainy season. These characteristics allow a P. juliflora seedling to grow fast in response to favorable water circumstances, such as rain, and to form roots before the soil dries out in the subsequent dry season. Furthermore, it was recorded that P. juliflora seedling may be able to establish itself in new habitats even during the dry season if its root system can access some water-rich areas of the soil during the rainy season [12]. Ecologists usually think that plant invasions are caused by three things: the number of propagules, how invasive the native community is, and how the land was used in the past, each factor might affect a specific habitat differently, and there might be connections between them [39]. However, soon after they were established, the trees rapidly encroached on agricultural and rangeland areas, lowering the productivity of the grazing and agricultural lands [12-14]. Previously it was reported that invasive species are common in semi-arid areas because of their specific environmental needs, such as the amount of light they need [40]. Recent studies concluded that the high amounts of ecosystem disturbance occurring in all kinds of habitats, including riparian ecosystems, rural farmland, urban greenbelts, wetland ecosystems, and forest ecosystems, facilitated the invasion of new species [6, 41-43].
Table 2.
Effect of the canopy of P. juliflora on the density (number of individuals per one hundred m2) for the associated species in North and south Jeddah.
Aridity Indices of the Study Area
The obtained data confirms that not only is the study area arid in general but also has become drier in the last 30 years. Aridity indices are numerical measures of the level of water scarcity at a certain location. Although several aridity indices have been developed, Thornthwaite’s 1948 study is expressly referred to when the term “aridity index” is used. Aridity indices have been used on both continents and subcontinents, and they are frequently connected to the distribution of wild vegetation and agricultural crops [44, 45]. The indices’ critical values were calculated using observed vegetation boundaries. It is well known that the area considered arid if Lang index less than 20, De Martonne index is less than 10 or/ and the Emberger index is less than 30 [30, 31]. The results strongly show that the study area is affected by climate change. This causes the Prosopis plant to spread more than the original plants because it can handle drought better.
Impact of P. juliflora on Soil Characters
It is well known that the expansion of invasive plants has an impact on the diverse, dynamic landscapes created by the intricate interactions between biotic and abiotic ecological processes [46]. In the current study, the invasion of P. juliflora caused a substantial (P = 0.05) fall in soil pH as well as an increase in organic matter, nitrogen, potassium, and phosphorus. P. juliflora’s ability to fix nitrogen could be the reason for excess nitrogen in the soil under the tree canopy, making soil closer to the tree canopy more fertile than soil farther away [47]. A previous study recorded that P. juliflora stands had significantly higher nitrogen, potassium, magnesium, calcium, and phosphorus nutritional content than other woody species [48, 49]. Decaying leaves and fruits can explain why there is so much organic matter, potassium, and magnesium in the soil under the tree. In other studies, it has been found that there are links between the type of soil and the types of plants that grow there. These connections can be explained by the fact that local edaphic factors affect the nutrient availability in various soil types, favoring plant communities with a variety of ecological roles [43, 50-52]. According to the results of a previous study [53], P. juliflora in this investigation increased the amount of phenolics in the soil. It was reported that P. juliflora’s dry leaves primarily contain phenolic compounds [53]. Because invasive and native species have different ways of staying alive, differences in form (the structure, composition, and life cycle strategy of plants), biomass, and litter can have a big effect on soil parameters [54]. Most of the research on how the invasion has changed the physical and chemical properties of the topsoil has been done on nitrogen, phosphorus, and carbon [49, 50]. As a consequence, both native and invasive species’ physiological processes have changed in this area, which may have an effect on how widely different species are distributed [55, 56]. Also, invasive plants may change the way that the soil’s mineral elements connect to each other [57].
Impact of P. juliflora on the Native Associated Species
The current study showed that P. juliflora plant has changed native species diversity and densities. Sometimes the P. juliflora caused the disappearance of many native species, such as finding that P. juliflora causes species to move and declines in species diversity and richness is consistent with many another research that confirmed the same results [7, 58-60]. According to the current research, most of the related native species, which are annual species, were found to have significantly lower densities because of the invasion of P. juliflora. Due to the exotic species’ superiority over native species in some measurable traits, such as dispersal and reproductive abilities, seedling survival and establishment, phenotypic plasticity, growth-related properties, plant height, and high susceptibility to herbivory and pathogens, native species have disappeared from the study area and the density of others has significantly decreased [61]. P. juliflora has a number of biological traits related to seed dormancy, germination, and dispersion that might speed up its colonization of new places [58-60]. Additionally, P. juliflora is a potent competitive invader because of its exceptional capacity for resprouting from stumped or injured trees with fast coppice development [62]. A previous study recorded that P. juliflora was described as fast-expanding, aggressive, and capable of degrading substratum in semi-arid and dry parts of the north and north-west of India [62]. P. juliflora has a high potential for invasion due to its rapid growth and numerous reproductive efforts. [62] confirmed that smaller P. juliflora individuals practically doubled in size in a year. The phenolics that the plant releases or the byproducts of their microbial transformation may play a role in P. juliflora’s capacity to inhibit the related species. However, other organic compounds could potentially be implicated in interacting with phenolics. In addition to their impacts on other plants, invasive plants’ allelochemicals can aid in the resistance to pests and diseases, giving them a competitive edge in their host area [63]. Additionally, phenolic allelochemicals can prevent plants from receiving nutrients from their environment and have an impact on their regular growth. Several plant species are suppressed when P. juliflora forms dense stands in Kenya [64] and in the United Arab Emirates [64].
In general, compared to other life forms, invasive shrub and tree species have a greater potential for survival and spread [66]. The study area’s high proportion of therophytes (56%) is consistent with earlier research in other Saudi Arabian regions [21, 67, 68]. Therophytes are a sign of desertification, severe human pressure from overgrazing, and ineffective land use management practices, which explain the high proportion of it in the associated species. They developed as a means of survival. These parallels demonstrated that most plants have an ecological niche-wide ruderal strategy. Therophytes are typically thought to be a sign of hot, dry regions [69]. Our research revealed striking parallels to [71], results about therophytes’ ability to withstand drought and high temperatures in arid environments. Therophytes evolved as a means of survival, are a sign of desertification and the severe human pressure brought about by overgrazing and poor land use management techniques. These similarities exhibited that most plants have a ruderal strategy with a wide ecological niche. Therophytes are generally considered to be a typical indicator of hot, dry climates [69]. Our findings showed significant similarities to Ahmed et al., (2020) who reported therophytes as a means of drought and high temperature resistance in arid environments.
Due to competition for resources, invasive species have an impact on local plant species and their surroundings [58]. They take up room and deplete soil nutrients, which hinders the growth of nearby vegetation. Rapid travel, the tourism sector, and increased international commerce are all significant factors causing the number of biotic invasions to steadily increase over time [59]. The Convention on Biological Diversity (CBD) says that invasive species from other places can be so bad for the environment that they are one of the main causes of biodiversity loss around the world [70]. Introduced outside of their native range, invasive plants can considerably contribute to the loss of biodiversity worldwide, among other unfavorable effects [71, 72]. Due to their capacity to significantly increase the number of viable offspring produced from the parent plant, AIPs have a major negative impact on the environment. This enables them to quickly devour vast areas [73].
Similar effects of the invasive shrub N. glauca on species richness and evenness were seen in the Taif area of western Saudi Arabia [74]. As a result, it’s possible that invasive species are already chosen to benefit from climatic change [75].
Conclusion and Recommendations
The invasive P. juliflora threatens native plants in the studied area and changes the chemical properties of the soil. Climate change increases the negative effects of P. juliflora. The results of this study recommend a strong need to manage and restrict the invasive P. juliflora, and greater plant diversity would be expected on these soils following its eradication.

