

Introduction
The salinity problem in irrigated land is described as a major environmental threat to crop production. It has been reported that soil salinity affects 20 to 50% of irrigated arable land [1]. Recently, the salinity has had an adverse effect on irrigated areas of approximately 2000 hectares in most of the regions, such as the Mediterranean shoreline located in the arid and semi-arid zones [2]. Moreover, one of the most important scenarios for the future in the regions dominated by the Mediterranean climate is the increase of soil salinity with the decrease of water resources [3]. Therefore, it is thought that salt-resistant plants will come to the forefront in the future.
Halophytic plants, known as salt-tolerant plants, are an important place in terms of capacity to respond to adverse effects caused by extraordinary environmental conditions. Marginal areas will be effectively used with the spread of such plants. Chenopodiaceae constitutes 44% of the class of halophytic plants, which host approximately 321 species [4]. Quinoa that provides extraordinary adaptation to harsh environments such as drought and salinity [5] is one of the most important members of the Chenopodium L. genus, which contains 150 subclasses, grown as annual and perennial [6].
The protein content of the quinoa plant (Chenopodium quinoa Willd.), which includes almost all essential amino acids [7], constitutes 13-19% of dry matter [8]. Furthermore, the quinoa plant, which has a relatively low proportion of calories, is considered a highly nutritious and healthy food ingredient [9] due to its high vitamin, mineral, and fiber content [10]. Quinoa, which is very important for vegans and vegetarians, is also a very important food source in livestock, including ruminant and poultry species [11].
A number of studies indicated that the effects of salinity stress on crops or their parts, such as biomass and dry matter changes or plant height, leaf size, leaf and steam thickness changes [12-16]. In the last few decades, some studies have focused on the effect of salinity on leaf anatomic properties such as leaf chlorophyll content, number of stomata, and size of stoma or parenchyma of quinoa [17-20], while other research has been conducted on how they respond to salinity stress from germination to the end of the seedling period [21]. Although it is known that quinoa varieties give different responses to salinity levels [22], there is almost no study focused on the response to salinity in the different varieties of quinoa [23].
Since the quinoa plant has a higher salt tolerance potential than other plants, it could be used for production in saline and alkaline soils [24]. However, it remains unclear whether some new quinoa varieties differ in their salt tolerance. In this study, the effects of five different levels of soil salinity on some characteristics were studied with a view to comparing two different varieties of quinoa, one old and the other new, during four different growth periods to approach closet information that appeared as a gap related to this subject in the literature.
Materials and Methods
Plant Material
The plant material of the study consisted of two quinoa varieties named “Saponinsiz” and “Valiente”. Prior to the experiment, twenty-five seeds from both cultivars were selected to ensure uniformity, and a viability test was performed for 7 days. So it was decided how many seeds to sow per pot.
Setting Up the Experiment and Salinity Treatments
In the study carried out in plant growth and development conditions with Mediterranean climatic conditions, only irrigation quantities were intervened. The standard field soil containing 2% of organic matter, 2978 mg kg-1 P2O5, 101 mg kg-1 exchangeable K, 19 mg kg-1 Ca, 5,6 mg kg-1 Na, 594 mg kg-1 Fe, and 21 mg kg-1 Mn was used in the present study. The experimental soil was put in pots with 50 L. The initial field capacity was calculated for randomly selected 3 pots. Eighty-five quinoa seeds were sown into the pots (April 5th, 2018). The number of plants was reduced to 70 in each pot immediately after the emergence of the plants from the soil (approximately twice of the sample number during the study to avoid sampling problems). The salinity treatments were applied afterward according to 8 dS m-1, 10 dS m-1, 12 dS m-1, 14 dS m-1, and 16 dS m-1 NACl concentrations, which were determined to be moderately salinity doses for quinoa varieties threatened (April 14th, 2018) with calculated water (measured EC value). The dose of water was based on the calculation which was made with the surface area of the pots. For each pot, 400 ml of water was supplied exclusively through surface irrigation once per week during the experimental period to prevent the reduction of the salt effect. Infiltration cases were placed under the pots against the possibility of infiltration. These processes were repeated again to 3 pots of each salt concentration (8 dS m-1, 10 dSm-1, 12 dS m-1, 14 dS m-1, and 16 dS m-1 NACl) and each variety (Saponinsiz and Valiente). Thus, the study was conducted with three replicates.
The traits studied in this research were determined in the following ways:
Daily maximum and minimum temperature values were measured during the months of the study (April, May, and June). According to these temperature values, Growing Degree-Days (GDD) values are calculated with the formula reported by [25]. Four different sampling dates were determined (April 30th, May 15th, May 29th, and June 12th) in view of the calculated GDD values (202.4 – 190.5 – 199.1 – 205.9). Then, seven full plants of each pot (salinity levels and varieties) were sampled in three repetitions on the same day (determined the dates) in 2018. Biomass, dry matter, leaf thickness, stomata number, stomata width, stomata length, and parenchyma length were measured on every sampling date.
Biomass: Randomly selected 7 plants from each pot were weighed. The weight of this labeled fresh or “green” biomass [26, 27]. The average was taken to obtain one of the replicate values (one of three repetitions) of salt concentrations and varieties.
Leaf thickness: The electronic compass was used to determine leaf thickness [28] in the plants, which was measured by biomass values. The plants were selected randomly for each repetition.
Dry matter: The plants randomly selected to measure biomass value (7 plants from each pot) were incubated at 70oC for 72 hours until complete dryness [29], and the dry samples were weighed. The average was taken to obtain one of the replicate values (one of three repetitions) of salt concentrations and varieties.
Leaf anatomical measurements (number of stomata, stomata length, stomata width, and parenchyma length): Three plants randomly selected from each pot were transferred to the laboratory in cold conditions to determine other leaf anatomical measurements (number of stomata, stomata length, stomata width, and parenchyma length). Other leaf anatomical measurements were achieved from a light research microscope (Olympus bx40) with a digital camera. The number of stomata cells (in per mm2) was defined in the mm2 area of the leaf sample surface according to methods reported by [30]. Stomata length (µm), stomata width (µm), and parenchyma length (µm) were measured as reported by [31] in the epidermal strip images, which are obtained by taking a profile from the epidermis of the leaf by light research microscope transferred to the computer screen [32].
Statistical Analysis
TARIST statistical software was employed to conduct variance analyses and to obtain least squares means for the investigated characteristics [33]. The analysis of variance (ANOVA) was employed to examine the differences between the quinoa cultivars and salt dose practices and the interactions between them. The significance of the differences between the means of the replications was tested using Fisher’s Least Squares Difference (LSD) at P≤0.05 probability [34].
Results and Discussion
The effect of 5 different salt concentrations on four different growth periods, including the germination up to the end of the seedling period, on biomass, dry matter, leaf thickness, stomata number, stomata width, stomata length, and parenchyma length values of two quinoa varieties (Saponinsiz and Valiente), was determined. As a result of a three-factor (growing period, cultivar, and salinity level) analysis of variance, we saw that the growing period, one of the sources of variance, was significant statistically in both its own and some of its interactions. The calculated mean squares with variance analyses separated by different growth periods are given in Table 1.
The values measured for different growth periods were analyzed and evaluated separately (Table 2 and Table 3). It can be seen that salinity level*cultivar interaction was significant for almost all values of the variance analyses (Table 1). Only leaf thickness values measured at four sampling stages, stomata width values measured at the third sampling stage (May 29th), and stomata length values measured at the second sampling stage (May 15th) were insignificant. Therefore, we proposed LSD (salinity level*cultivar) values additionally, as shown in Tables 2 and 3). Moreover, we interpreted the dry matter and biomass values graphically (Fig. 1 and Fig. 2) because of better understanding.
Changes in biomass values of quinoa varieties (Saponinsiz and Valiente) under different salinity levels during growth periods are shown in Fig. 1. The final data revealed that maximum biomass values were obtained when plants were exposed to 10 dS m-1 for Saponinsiz (1,0 g) and 8 dS m-1 for Valiente (1,0 g) cultivars on April 30th. For the second sampling date (May 15th), maximum biomass values were obtained from 14 dS m-1 for Saponinsiz (1,1 g) and 12 dS m-1 for Valiente (1,7 g) cultivar. For the last two sampling times, maximum biomass values were obtained from 12 dS m-1 for Saponinsiz (4,5 g) and 10 dS m-1 for Valiente (3,8 g) cultivars on May 29th, 14 dS m-1 for the Saponinsiz (7,0 g), and 12 dS m-1 for the Valiente (9,9 g) cultivars on June 12th. Although it has been observed that different salinity levels for maximum value of biomass between the varieties on all sampling dates appeared, minimum values of biomass were obtained from usually 16 dS m-1 salinity level.
Table 1.
The calculated mean squares with variance analysis.
Table 2.
Leaf thickness, stoma number, stoma width, stoma length and parenchyma length values under different salt levels on the first and second sampling stages.
Table 3.
Leaf thickness, stoma number, stoma width, stoma length and parenchyma length values under different salt levels on the third and fourth sampling stages.
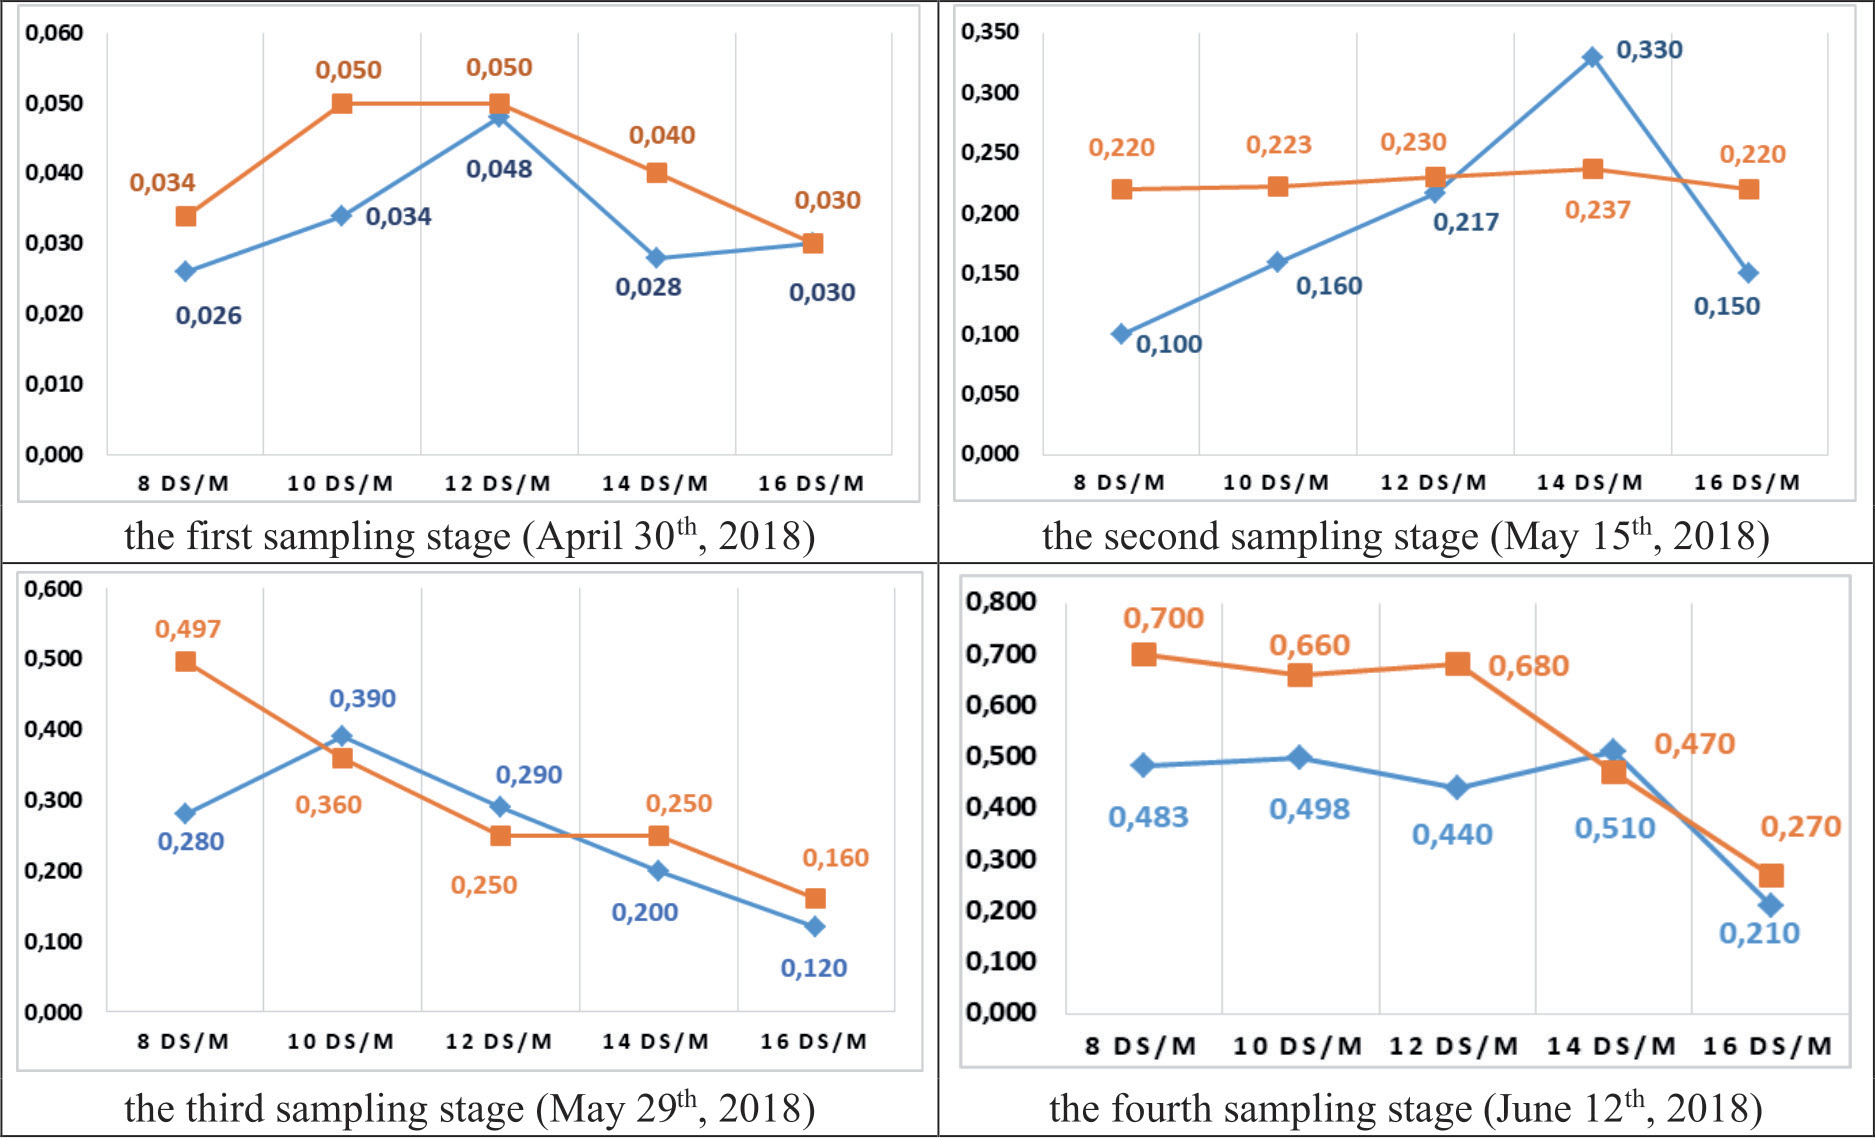
Changes in dry matter values of quinoa varieties (Saponinsiz and Valiente) under different salinity levels during growth periods are shown in Fig. 2. Maximum dry matter values were obtained from 12 dS m-1 for both Saponinsiz (0,05 g) and Valiente (0,050 g). Moreover, the Valiente cultivar demonstrated a maximum dry matter value of 10 dS m-1 (0,05 g) on April 30th. Moreover, maximum dry matter values were obtained from 14 dS m-1 for both Saponinsiz (0,33 g) and Valiente (0,24 g) on May 15th. For the last two sampling dates, maximum dry matter values were obtained from 10 dS m-1 for Saponinsiz (0,390 g) and 8 dS m-1 for Valiente (0,50 g) on May 29th, from 14 dS m-1 (0,51 g) for Saponinsiz and 8 dS m-1 (0,27 g) for Valiente on June 12th. Similar results of the biomass value: large decreases were observed in dry matter values under 16 dS m-1 for two varieties.
The response of the quinoa varieties to salinity treatment during growing periods was variable during the early sampling stages (Fig. 1 and Fig. 2). According to biomass and dry matter values, quinoa varieties (Saponinsiz and Valiente) could be resisted at 8 dS m-1 and 10 dS m-1 during four different growth periods. But Saponinsiz showed maximum biomass and dry matter value under a dose of 14 dS m-1 at the last sampling stage. Previous findings have shown that salinity reduces plant water consumption, nutrient uptake, cell turgor pressure, stomatal conductance, transpiration, and photosynthesis [35-37], resulting in greater reductions in yield, biomass, and dry weight [38-40]. Our results were slightly different because the quinoa plant is a typical halophyte [41]. There were indications that the salt tolerance of the Saponinsiz variety is more resistant than Valiente to increasing doses of salt over time. Moreover, many studies have determined a correlation between dry matter [42-44], biomass [17, 45], and grain yield [46-48]. Therefore, our results can be considered as concrete evidence of high yield values at the salinity levels.
Leaf thickness, stomata number, stomata width, stomata length, and parenchyma length values under different salt concentration levels on growth periods were shown as the first sampling stage values in Table 2 and Table 3.
Maximum leaf thickness of the Saponinsiz variety was obtained from 10 dS m-1 (0,63 mm) on April 30th, 8 dS m-1 (0,36 mm) on May 15th, 10 dS m-1 (0,39 mm) on May 29th, and 14 dS m-1 (0,15 mm) on June 12th. The highest values of Valiente were listed as 14 dS m-1 (0,59 mm), 12 dS m-1 (0,40 mm), 12 dS m-1 (0,45 mm), and 12 dS m-1 (0,19 mm), respectively, in terms of leaf thickness.
Fig. 1.
Changes of biomass (g) values of quinoa cultivars (Saponinsiz and Valiente) under different salinity levels during growing periods.
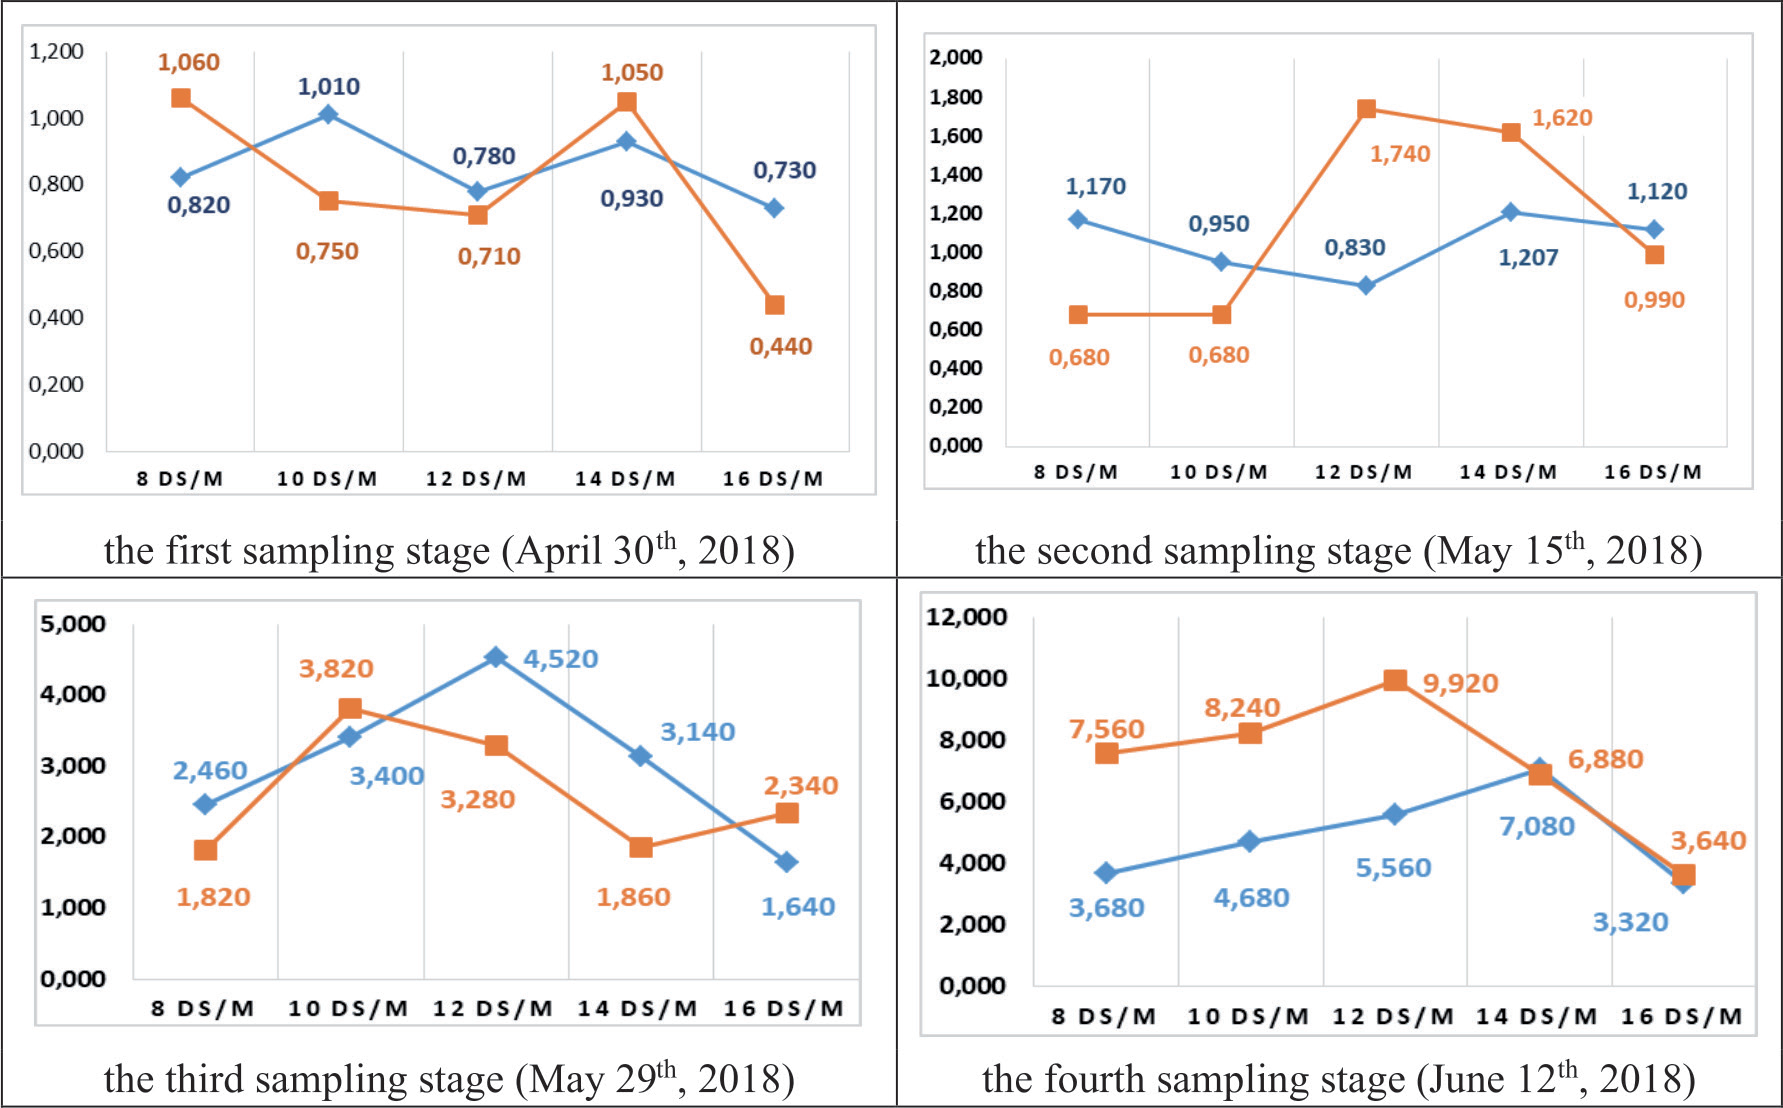
Fig. 2.
Changes of dry matter (g) values of quinoa cultivars (Saponinsiz and Valiente) under different salinity levels during growing periods.
According to the leaf thickness data obtained from all sampling dates, we would suggest that varieties showed different reactions against increasing salt doses during the growth periods (from sampling stage 1 to 4). Although the maximum leaf thickness value of Saponinsiz was obtained from increasing salt concentrations up to 14 dS m-1 during the growth periods, the maximum value of Valiente decreased. Increased leaf thickness has been reported as a successful trait for plant species growing under saline conditions [49]. Leaf thickening is considered a mechanism to increase water retention by mesophyll tissues in order to counteract salt toxicity [50]. The leaf thickness and leaf succulence significantly increased as the percentage of salinity increased [51]. Leaf thickness was considerably higher in the leaves of high salt treated plants [52], due to increased leaf thickness by limited water passing and the constraints to save water rendering the leaves succulent. Thus, increased leaf succulence by salt sequestration within the hypodermal tissue was a salt managerial method [53]. We may approach the fact that Saponinsiz is more resistant to salinity levels up to 14 than the Valiente cultivar in the following growth periods.
Maximum stomata number values of the Saponinsiz variety were obtained from 12 dS m-1 (15,45) on April 30th, 8 dS m-1 (41,20) on May 15th, 8 dS m-1 (43,10) on May 29th, and 8 dS m-1 (44,27) on June 12th. The maximum values of Valiente were listed as 8 dS m-1 (8,38), 8 dS m-1 (47,13), 8 dS m-1 (71,13), and 8 dS m-1 (70,50), respectively. Maximum stomata width values of Saponinsiz were obtained from 16 dS m-1 (0,049 µm) on April 30th, 12 dS m-1 (0,05 µm) on May 15th, 8 dS m-1 (0,05 µm) on May 29th, and 8 dS m-1 (0,05 µm) on June 12th. The salt doses that showed the maximum values of Valiente were listed as 14 dS m-1 (0,06 µm), 12 dS m-1 (0,05 µm), 10 dS m-1 and 12 dS m-1 (0,05 µm), and 12 dS m-1 (0,06 µm), respectively. Maximum stomata length values of Saponinsiz were obtained from 14 dS m-1 (0,08 µm) on April 30th, 12 dS m-1 (0,09 µm) on May 15th, 14 dS m-1 (0,09 µm) on May 29th, and 14 dS m-1 (0,09 µm) on June 12th. The salt doses that showed the maximum values of Valiente were listed as 16 dS m-1 (0,10 µm), 12 dS m-1 (0,10 µm), 10 dS m-1 level (0,10 µm), and 10 dS m-1 (0,10 µm), respectively. Maximum parenchyma length values of Saponinsiz were obtained from 12 dS m-1 for Saponinsiz (0,30 µm) on April 30th, 8 dS m-1 (0,35 µm) on May 15th, 8 dS m-1 (0,40 µm) on May 29th, and 8 dS m-1 (0,46 µm) on June 12th. The maximum values of Valiente were listed as 14 dS m-1 (0,27 µm), 8 dS m-1 (0,46 µm), 10 dS m-1 (0,35 µm), and 10 dS m-1 (0,36 µm), respectively.
Stomata are the morphological structures that control photosynthesis and transpiration. In general, characteristics of stomata vary greatly among genotypes and growth periods [54]. According to data from stomata number, stomata width, stomata length, and parenchyma length, quinoa varieties showed a few similar responses to increasing salt doses during the growth periods (from sampling stage 1 to 4), unlike leaf thickness values. The varieties were more affected by increasing salt doses during plant growth. Initially, maximum stomata size and parenchyma length values were obtained from high salt levels such as 14 dS m-1 or 16 dS m-1, the salt level at which maximum stomata size (stomata length and width) and parenchyma length values were obtained decreased with continued growth periods. Stomata number value decreased with increasing salt levels in each sampling stage. For almost all growth periods of the study, maximum stomata number values were obtained from the lowest salinity level. Low stomata density has been recognized as an adaptive trait to cope with saline stress [55]. An increase in stomata area has been linked to both enhanced stomata conductance and higher water use efficiency [19]. The reduction of stomata size under saline conditions may be recognized as a strategy to diminish the leaf water loss [56]. Because of the ability of plants to be able to regulate the size of the stomata opening, this is a very significant mechanism to control water loss. This ability is important during stressful conditions when loss of water can have serious consequences for the plants. These parameters can provide adaptation to salt stress by decreasing the stomata width and index, and thus by reducing the transpiration [57]. The process of photosynthesis takes place mainly within palisade cells, and then an increased thickness of the palisade parenchyma allows higher photosynthetic activity [58] and also greater production of carbohydrates [50]. While various parameters can be used to evaluate a plant’s ability to overcome salt stress, such as seed germination, biomass and dry matter values, and leaf photosynthetic capacity, leaf anatomy has been found to be a key factor in this process [59]. Salt-tolerant plants have changed the leaf anatomy firstly to protect themselves from environmental pressures [19]. This is particularly important in the context of salt stress induced osmotic stress, which can lead to water loss from plant leaves [60-62]. So, the structure of quinoa leaves plays a crucial role in limiting non-stomatal water loss [55, 63, 64]. The results can also provide a valuable perspective into the resistance of different quinoa varieties to water shortages caused by salt based on their leaf structure. If we ignored the first sampling stage, we could say that the Saponinsiz and Valiente varieties have higher parenchyma length values than 14 dS m-1 or 16 dS m-1. Furthermore, it may say that they were resisting all salinity levels except 14 dS m-1 or 16 dS m-1.
Conclusions
Salt tolerance in plants is a complex mechanism, and different plant species have different strategies to survive salt stress. In the present study, we analyzed and compared the morphological and some leaf anatomical characteristics responses of quinoa varieties from different habitats to salt stress. The study provided detailed and accurate information on the influences of different salt doses on the quinoa plant in Mediterranean climate conditions. The results are listed below. – Varieties of quinoa (Saponinsiz and Valiente) used in work have demonstrated the ability to be resistant at 8 dS m-1 - 10 dS m-1 as the limit of salinity values for general field crops. Both varieties have shown the best performance of almost all the properties (except for stomata size). Moreover, the Saponinsiz variety has also shown the best performance of dry matter and biomass and showed good performance of almost all the properties at higher salt doses (12 dS m-1 - 14 dS m-1) in the later growing period (sampling stages 3-4). This research showed that different cultivars of a crop might show different responses to salinity throughout the growing period, including four different growth periods covering the germination until the end of the seedling stage (April 30th, May 15th, May 29th, and June 12th). We could suggest the Saponinsiz variety for almost all salinity levels of the study (except 16 dS m-1). If soil salinity levels are up to 10 dS m-1, you should examine differences between the two varieties in terms of other parameters such as seed quality. – Even if some quinoa varieties such as Titicaca observed a significant inhibitory effect on seed germination for concentrations higher than 40 dS m-1 NaCl, quinoa optimal plant growth was obtained between 10 dS m-1 and 20 dS m-1 NaCl. We can say that the Saponinsiz and Valiente varieties tolerated moderately saline conditions under the Mediterranean climate. Therefore, in Mediterranean shorelines located in the arid and semi-arid regions in which water or soil is saline and other regions of the world affected by salt under Mediterranean climate conditions, tolerant cultivars that resist moderate salinity conditions should be sown for sustainable agriculture and beneficial income.

