

Introduction
In recent years, the recycling and utilization of kitchen waste have gained significant attention due to environmental concerns [1]. Current methods for composting food and kitchen waste primarily include feed production, composting, and biodiesel extraction [2-4]. Compared to traditional incineration and landfill methods, these approaches offer significantly better environmental benefits [1, 5]. Among them, kitchen waste composting not only reduces urban waste but also produces organic fertilizers with nutritional value [6]. The composting of kitchen waste has found some applications in agriculture, notably achieving success primarily in rice cultivation [7]. Additionally, some researchers have explored its partial substitution for peat in vegetable seedling cultivation, yielding certain positive results [8]. However, it has not yet achieved significant replacement of peat by composted kitchen waste, with the highest substitution level reaching only 10% [9]. It is important to acknowledge that substituting peat with kitchen waste compost for seedling substrates is feasible and promotes resource recycling with economic and ecological benefits [10-12]. However, high salt levels (Na+ and Cl-) in kitchen waste compost can hinder seed germination and seedling growth [13]. To mitigate this, two approaches are used: improving compost properties through extensive rinsing and adding organic materials, or incorporating exogenous substances like sulfur powder and plant growth regulators to enhance seedling tolerance to saline-alkali stress [14].
Bacillus spp., widely found in natural environments, influences plant growth and development through various biological characteristics and metabolic functions [15, 16]. They decompose organic matter into plant-absorbable nutrients, enhancing nutrient utilization efficiency [17, 18]. Additionally, substances produced by Bacillus spp., such as auxins and gibberellins, stimulate plant growth and improve stress resistance [19]. Previous studies have shown positive effects of B. subtilis, B. amyloliquefaciens, and B. velezensis on tomato plant growth, yield, and resistance to bacterial wilt [20]. Consequently, the application of Bacillus in agricultural production processes is increasingly prevalent. The most common approach involves using Bacillus to produce bio-organic fertilizers, which have shown significant improvements in crop yield, quality, and disease resistance [21, 22]. Additionally, Bacillus has been used in the preparation of seedling substrates. However, it remains uncertain whether Bacillus can effectively alleviate the toxic effects of salt on seed germination and seedling growth in kitchen waste composting. This prompted us to explore whether adding these three Bacillus spp. to seedling substrates would positively impact seedling quality. Therefore, based on prior research, our study investigates the effects of B. subtilis, B. amyloliquefaciens, and B. velezensis inoculation on cucumber seedling growth, substrate chemical properties post-seedling, and pathogen quantity in substrates prepared from kitchen compost, aiming to provide scientific evidence and technical support for agricultural production.
Experiment
Test Materials
The experimental substrate was prepared by mixing kitchen waste compost with peat, vermiculite, and perlite in 10%:40%:40%:10% volume ratio. The initial substrate properties included a pH of 7.57, electrical conductivity was 1.25 mS·cm-1, alkali nitrogen content was 1.22 g·kg-1, available phosphorus content was 1.14 g·kg-1, soluble potassium content was 1.96 g·kg-1, and organic matter content was 22.73%. B. subtilis, B. amyloliquefaciens, and B. velezensis were provided by the Microbial Research Laboratory of Anhui Agricultural University. The test crop used for seedling cultivation was cucumber, specifically the cultivar JinYan 4.
Preparation of Strain Cultures
Three strains of Bacillus spp. were streaked onto Nutrient Agar (NA) plates and incubated at 28ºC for 48 hours. The activated strains were then inoculated into 250 mL Erlenmeyer flasks containing 100 mL of Nutrient Broth (NB) and incubated at 28ºC with shaking at 150 rpm for 72 hours to obtain the bacterial culture broth. Subsequently, the bacterial culture broth was inoculated into 250 mL Erlenmeyer flasks containing 90 mL of culture medium at a ratio of 5% and incubated at 28ºC with shaking at 180 rpm for 96 hours to obtain the bacterial culture solution, which was stored at 4ºC for further use.
Experimental Design
The seedling substrate was conducted using a 50-cell seedling tray with compost prepared from kitchen waste. One seed was sown per cell at a depth of 0.5 cm from the surface of the compost. Four treatments were established, each with three replicates, and each seedling tray constituted one replicate. Each replicate was irrigated with 1.5 L of water, with plain water used as the control (CK), and the remaining treatments receiving irrigation with B. subtilis, B. amyloliquefaciens, and B. velezensis culture solutions, denoted as T1, T2, and T3, respectively. The trays were placed in a growth chamber maintained at 25°C and 80% humidity for 15 days, with additional watering applied as necessary throughout the experimental period.
Measurement Items and Methods
Seedling Growth
Ten days after sowing, the number of emerged cucumber seedlings was counted to calculate the seedling emergence rate and cotyledon emergence rate. Additionally, the leaf area of cucumber seedlings was determined using the leaf area coefficient method [23]. Fifteen days after sowing, fifteen healthy cucumber seedlings per tray were selected for morphological measurements. The height of seedlings was measured using a ruler, while stem diameter was measured using a vernier caliper. Chlorophyll content was determined using a chlorophyll meter, expressed as SPAD values, on fully expanded leaves. The leaf area of cucumber seedlings was also measured. Furthermore, the substrate adhered to the roots of the selected cucumber seedlings was collected using a brush, sealed, and stored at 4ºC for subsequent analysis.
Then root length and root surface area of cucumber seedlings were determined using a root scanner. The fresh weight of both above-ground and below-ground parts of cucumber seedlings was measured using an electronic balance. Subsequently, samples were dried at 60ºC to a constant weight, and dry weights were recorded to calculate the seedling vigor index. The growth performance of cucumber seedlings under different substrate compositions was evaluated using the membership function method [14]. Higher membership values indicate better growth of cucumber seedlings under the respective substrate composition. The membership values and seedling strong index were calculated using the following formulas:
Where i denotes the treatment and j denotes the seedling growth indicator; Xij denotes the measured value of the j indicator under treatment i; Xjmax denotes the maximum value of the j indicator in each treatment; and Xjmin denotes the minimum value of the j indicator in each treatment.
Chemical Property
The substrate adhering to cucumber seedlings was air-dried, ground, and sieved through a 2 mm mesh, following the methods specified in the agricultural industry standard “NY/T 2118-2012 Vegetable Seedling Substrate”[9]. The chemical properties of the substrate were then determined, including pH value, EC value, and contents of alkali-hydrolyzable nitrogen, available phosphorus, quick-acting potassium, and organic matter, in accordance with the aforementioned standard.
Quantitative Fluorescence Analysis of Fusarium spp.
Cucumber seedlings attached to nursery substrates were utilized as analysis samples. The genomic DNA of the samples was extracted using the CTAB method and served as the template for qPCR. The extracted DNA was eluted in 40 μL of Tris-HCl buffer (pH 8.0) and stored at -20ºC for subsequent analysis. Real-time qPCR analysis was performed using specific primers ITS-Fu-f and ITS-Fu-r targeting the fungus Fusarium oxysporum. The amplification protocol was adapted from Meng et al. [24].
Data Statistics and Analysis
Using DPS 18.1 software [25], the trial’s raw data were submitted to one-way ANOVA after being tallied using Excel 2019.
Results
Seedling Growth
The investigation into the emergence of cucumber seedlings 10 days after sowing revealed various effects. As shown in Table 1, different strains of Bacillus had no significant impact on the emergence rate of cucumber seedlings. However, they significantly increased the cotyledon rate and leaf area compared to the control (CK) (P<0.05), with no significant differences observed among the Bacillus treatments. Specifically, the cotyledon rate increased by 105.07% to 112.16%, and the leaf area increased by 7.76% to 11.26% relative to CK.
Regarding the aboveground growth indicators of cucumber seedlings, different strains of Bacillus exhibited variations in different growth parameters. B. subtilis (T1) and B. velezensis (T3) significantly outperformed CK and B. amyloliquefaciens (T2) in chlorophyll content (Fig. 1c), leaf area (Fig. 1d), aboveground fresh weight (Fig. 1e), and aboveground dry weight (Fig. 1f) (P<0.05). However, there were no significant differences between T2 and CK in these four parameters. T2 showed the highest plant height at 2.78 cm, representing a 9.88% increase over CK. T1 and T3 exhibited the best performance in chlorophyll content and aboveground dry weight, surpassing CK by 18.13% to 21.14% and 54.37% to 55.17%, respectively. T3 excelled in leaf area and aboveground fresh weight, showing increases of 69.30% and 64.03% relative to CK. In terms of stem thickness, all Bacillus treatments were significantly better than CK (P<0.05), but there were no significant differences among the Bacillus treatments.
Table 1.
Effect of different Bacillus species on the emergence of cucumber seedlings.
| Treatments | Seedling rate/% | Central leaf rate/% | Cotyledon area/cm2 |
|---|---|---|---|
| CK | 80.00±6.93a | 42.83±2.88b | 7.99±0.26b |
| T1 | 85.33±2.91a | 87.89±2.87a | 8.61±0.45a |
| T2 | 87.33±1.76a | 90.87±1.15a | 8.62±0.83a |
| T3 | 85.33±2.91a | 87.83±4.52a | 8.89±0.79a |
Fig. 1.
Effect of different Bacillus species on the above-ground growth of cucumber seedlings. Note: Different lowercase letters in the same column represent significant differences (P<0.05). CK represents the blank control, while T1, T2, and T3 represent Bacillus subtilis, Bacillus amyloliquefaciens, and Bacillus velezensis, respectively.
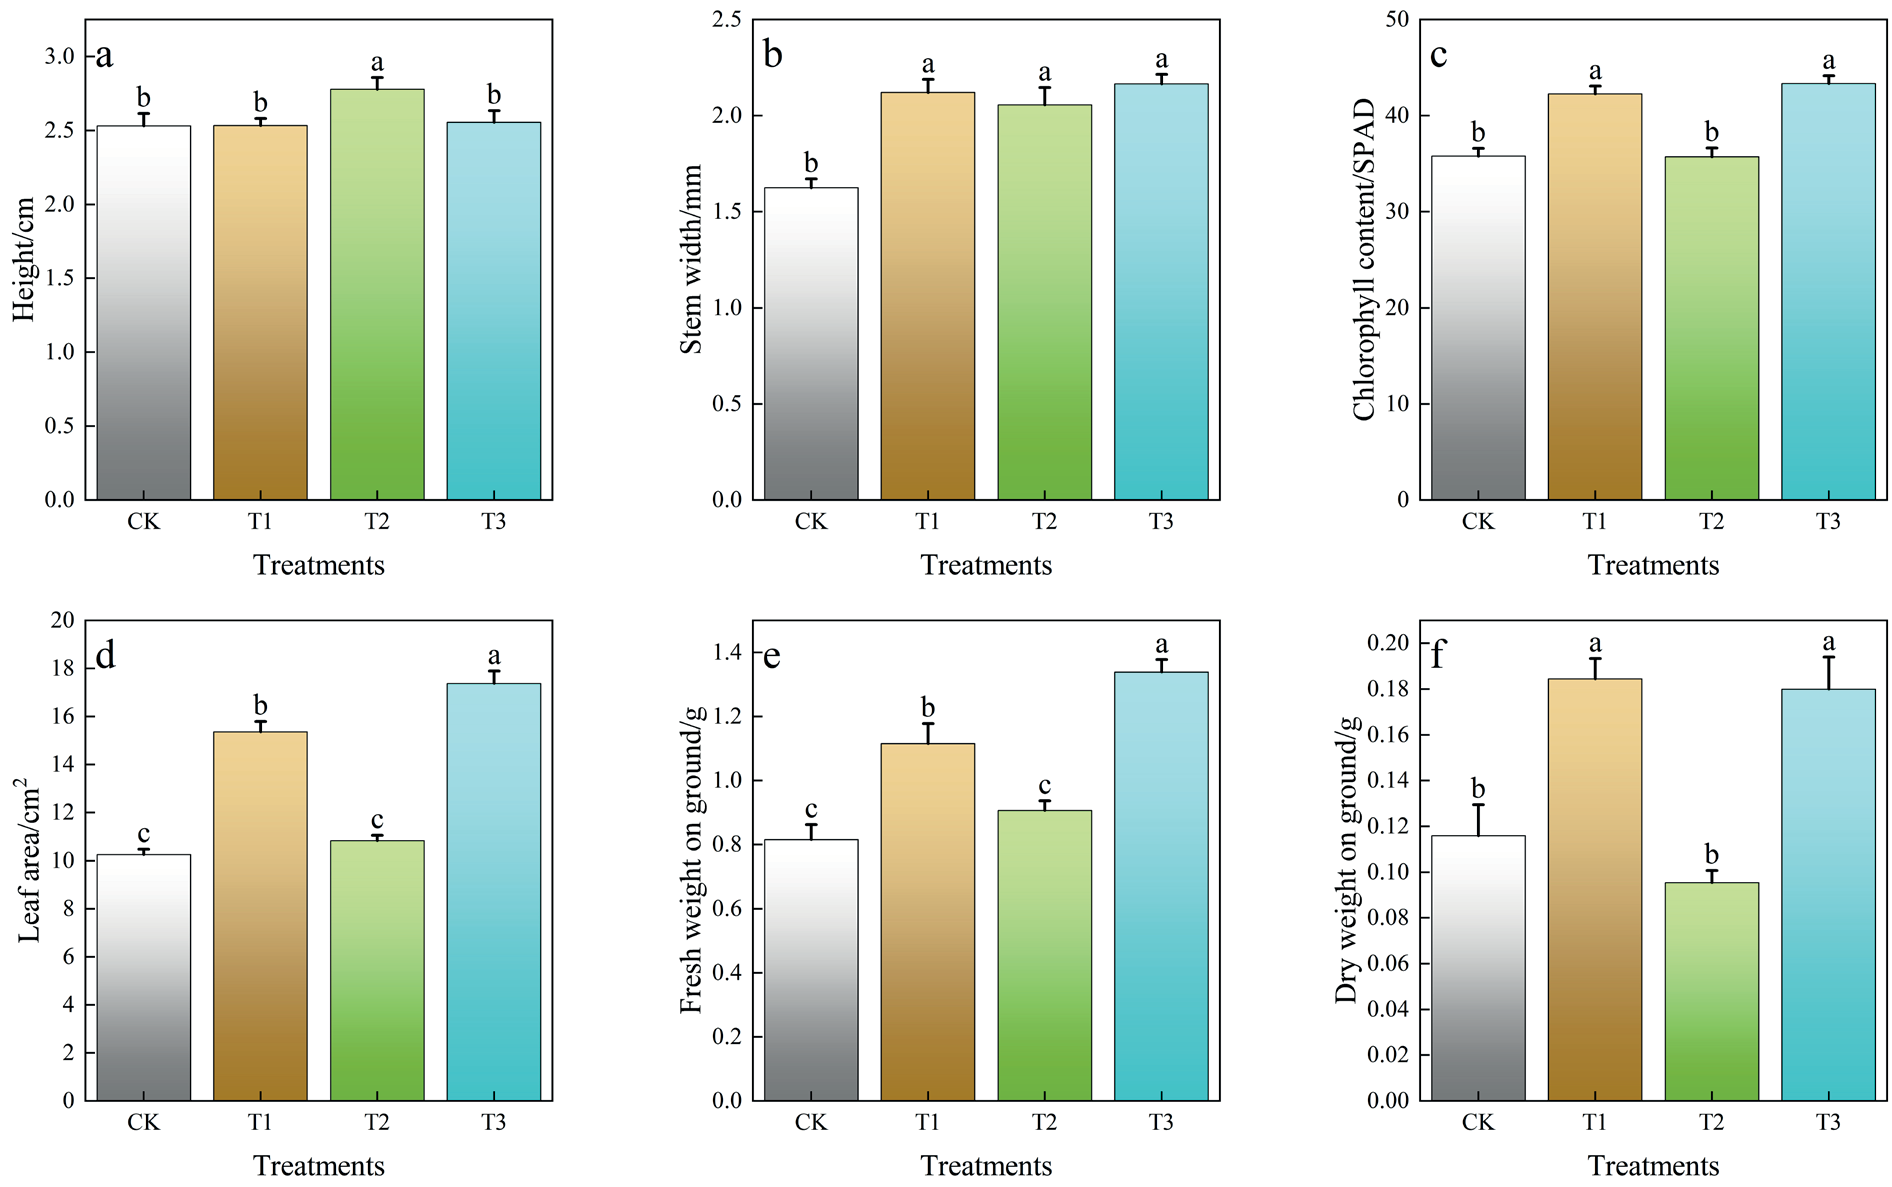
Fig. 2.
Effect of different Bacillus species on the below-ground growth of cucumber seedlings. Note: Different lowercase letters in the same column represent significant differences (P<0.05). CK represents the blank control, while T1, T2, and T3 represent Bacillus subtilis, Bacillus amyloliquefaciens, and Bacillus velezensis, respectively.
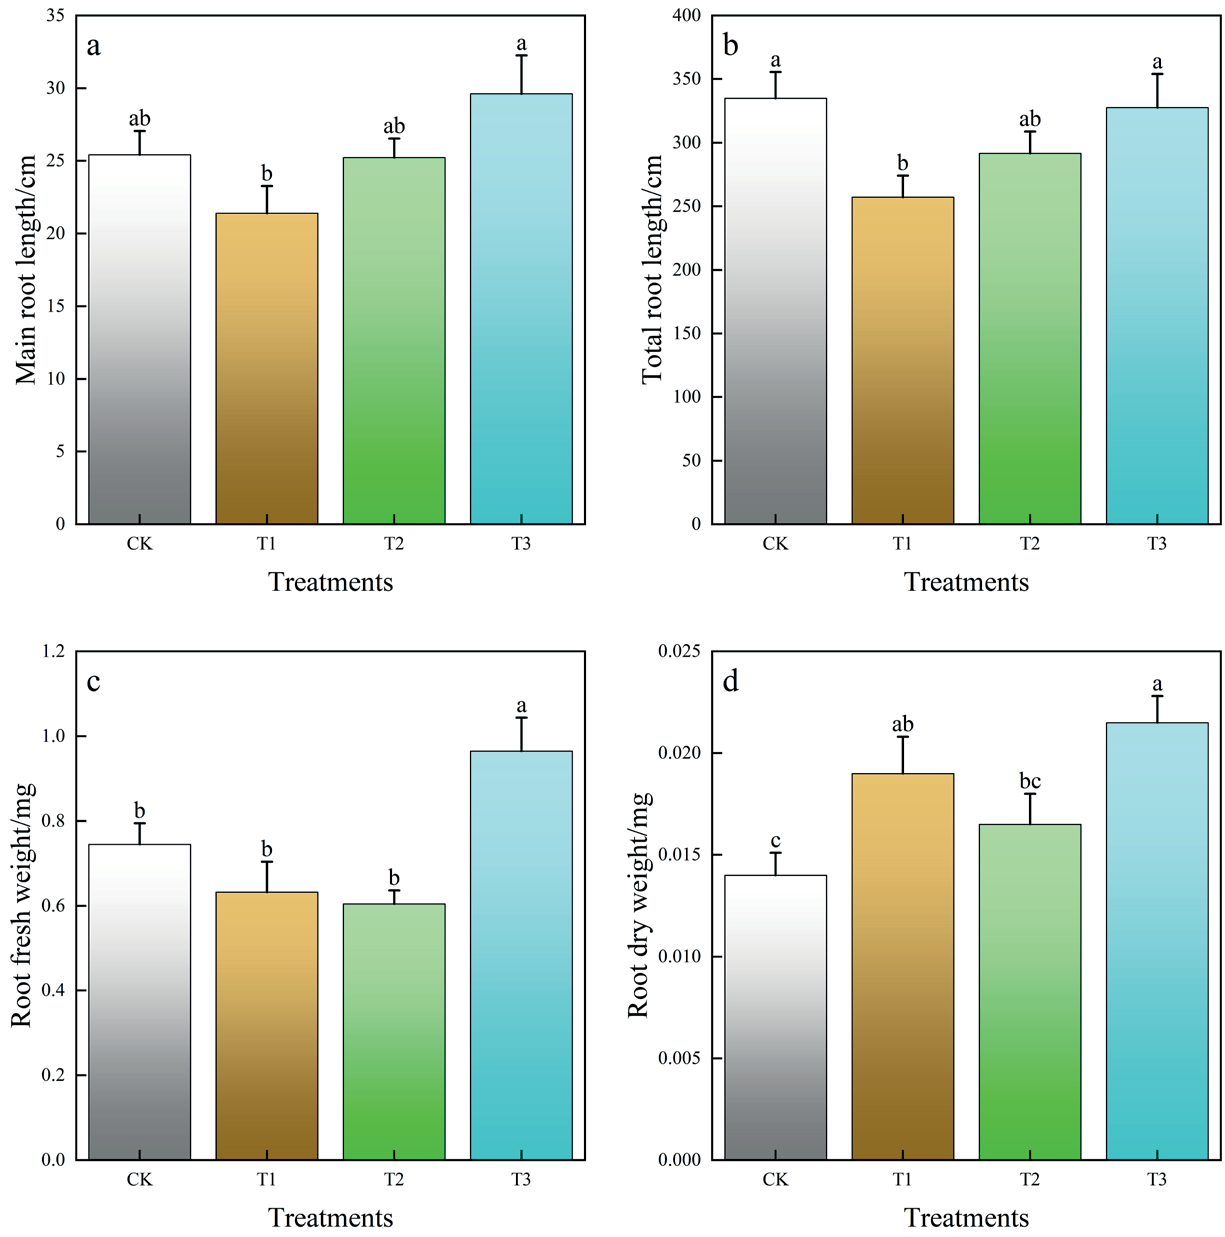
In terms of underground growth of cucumber seedlings, T1 and T2 did not demonstrate superiority in root length (Fig. 2a), total root length (Fig. 2b), and underground fresh weight (Fig. 2c) compared to other treatments. However, T3 significantly outperformed CK in underground fresh weight and dry weight (Fig. 2d). Specifically, T3 exhibited a 29.62%, 52.69%, and 59.64% increase in underground fresh weight compared to CK, T1, and T2, respectively. Despite the pronounced promotion of aboveground growth, especially in promoting effects, the three strains of Bacillus did not show significant promotion effects on underground growth, particularly in root length.
Comprehensive Evaluation of Seedling Growth
Considering the varied performance of the three Bacillus strains on numerous growth indicators of cucumber seedlings, this study employed the seedling strong index and the fuzzy membership function method to comprehensively evaluate the growth status of cucumber seedlings. As shown in Table 2, both T1 and T3 significantly outperformed CK and T2 in terms of the seedling strong index. However, it remained challenging to distinctly differentiate the superiority or inferiority among the four treatments. Regarding the average membership degree, the four treatments can be ranked in the following order based on their average membership degree: T3>T1>T2>CK. A higher average membership degree indicates a better growth-promoting effect of the corresponding treatment on cucumber seedlings. Thus, it is evident that T3 exhibits the most optimal growth-promoting effect on cucumber seedlings.
Chemical Property
Bacillus spp. proliferate within the substrate, potentially inducing alterations in its chemical properties. As depicted in Fig. 3, the pH of the substrate remained relatively stable across all treatments (Fig. 3a), ranging from 7.36 to 7.52. However, a noticeable increase in the substrate’s Electrical Conductivity (EC) was observed. Treatment T1 exhibited significantly higher EC values, chloride ion (Cl-) content, and sodium ion (Na+) content compared to the other three treatments. Given that the seedling substrate utilized in this study was partially composed of kitchen compost, additional attention was directed toward chloride and sodium ions to mitigate excessive salt incorporation into the soil during transplanting. Fig. 3c and 3d indicate that CK, T2, and T3 did not significantly differ in sodium and chloride ion content, suggesting that B. subtilis and B. velezensis may not facilitate the absorption of these ions by cucumber plants.
Fig. 3.
Effect of different Bacillus species on the chemical properties of the post-nursery substrate. Note: Different lowercase letters in the same column represent significant differences (P<0.05). CK represents the blank control, while T1, T2, and T3 represent Bacillus subtilis, Bacillus amyloliquefaciens, and Bacillus velezensis, respectively.
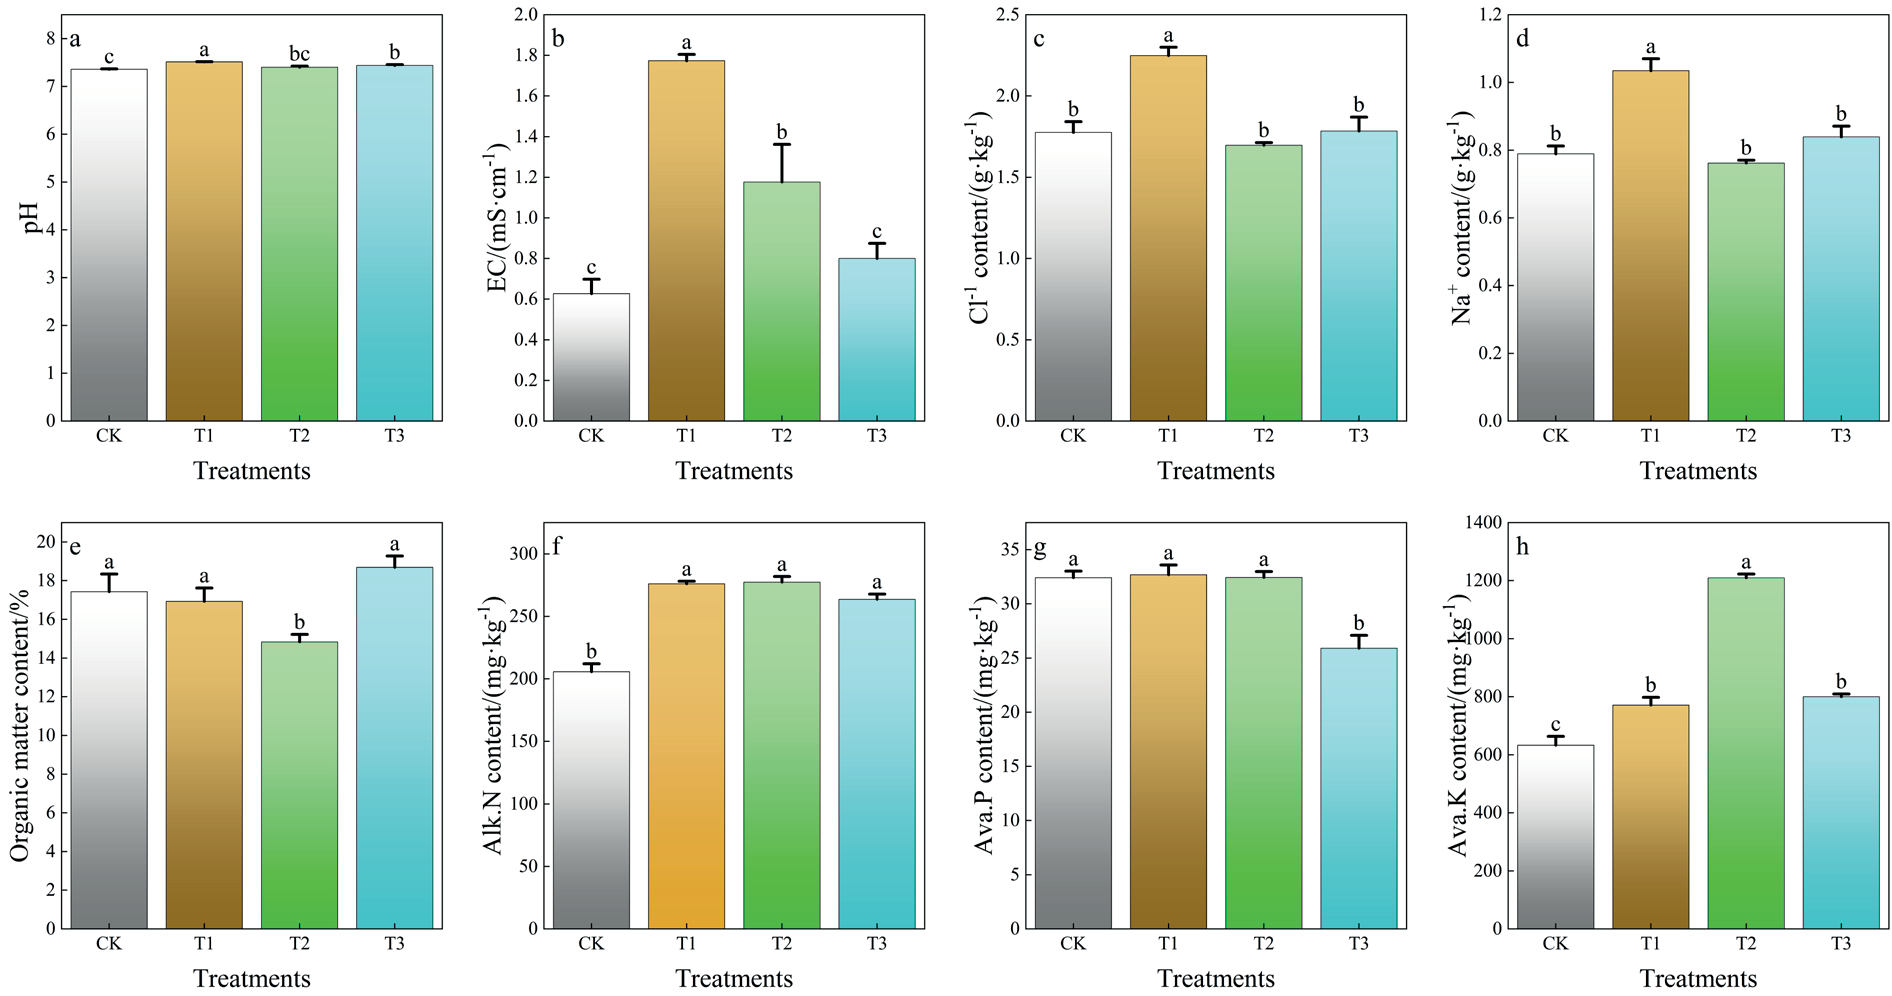
Regarding nutrient content in the seedling substrate, Bacillus spp. significantly enhanced the levels of mineralized nitrogen (Fig. 3f) and available potassium (Fig. 3h) compared to the control (CK). This enhancement could be attributed to the microbial breakdown of organic matter within the seedling substrate, resulting in increased nutrient content relative to the control. However, in terms of available phosphorus content, T3 exhibited a significant decrease compared to the other treatments, and T2 showed significantly lower organic matter content than the other treatments.
Microbiological Content of Fusarium spp.
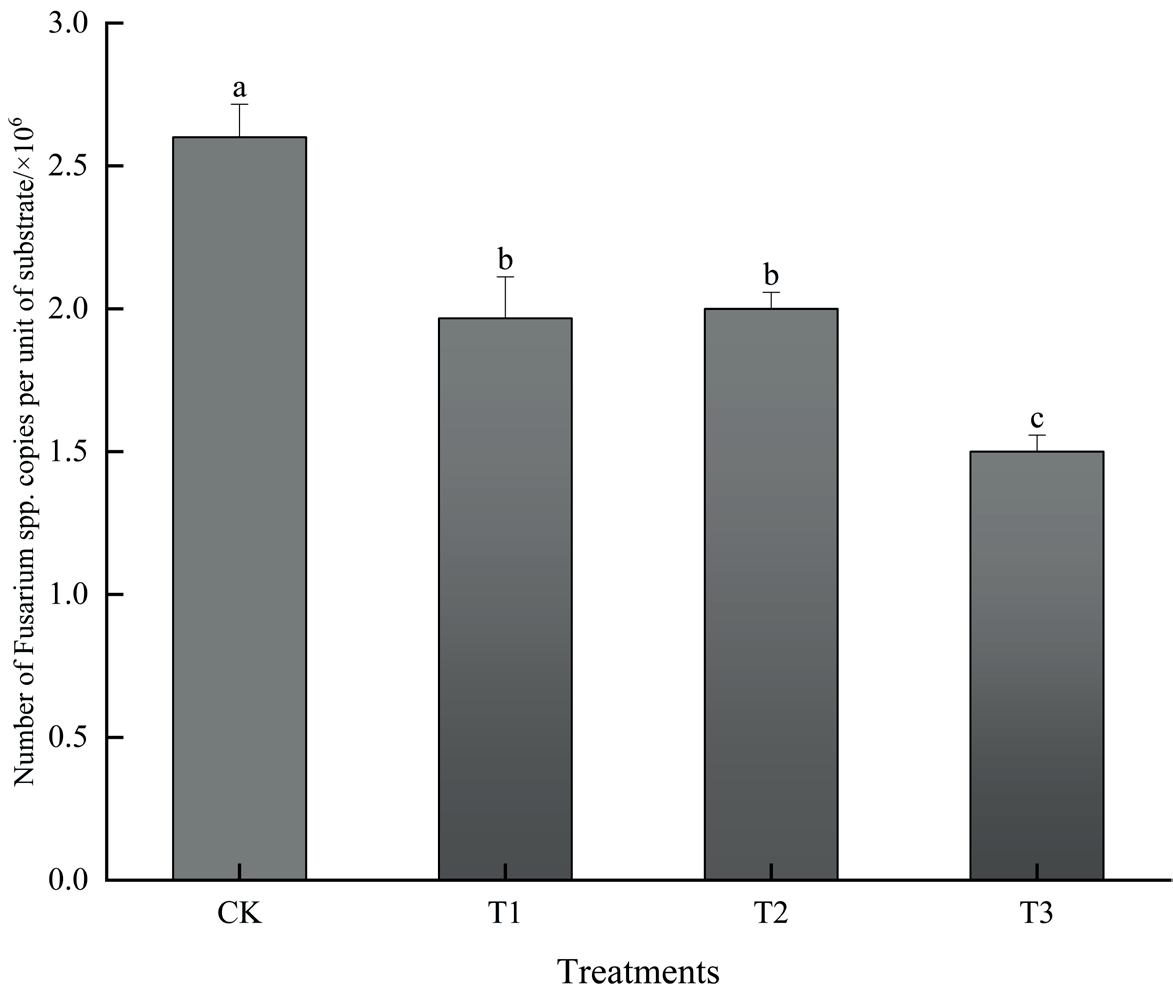
The microorganisms of the Fusarium genus are significant contributors to various soilborne diseases, including wilt disease, in cucumbers. The addition of B. subtilis significantly reduced the abundance of Fusarium genus microorganisms within the seedling substrate (Fig. 4), with the most pronounced effect observed in treatment T3. Compared to the control (CK) and treatments T1 and T2, T3 reduced Fusarium genus microorganism content by 42.31%, 23.73%, and 25.00%, respectively, effectively suppressing the occurrence of soilborne diseases during the cucumber seedling stage.
Discussions
The main challenge of using kitchen waste compost is its unstable properties, which necessitate careful management to avoid significant variations in substrate quality [26]. Adding 10% kitchen waste compost to seedling substrates, as done in this study, has shown promising results but also occasional issues with underground diseases like wilt. Incorporating B. subtilis, B. amyloliquefaciens, and B. velezensis into the substrate significantly reduced Fusarium populations, partially controlling underground diseases. Additionally, these B. strains promoted cucumber seedling growth, particularly in aboveground parts, highlighting their potential to improve seedling quality in compost-based substrates. Kitchen waste compost contains high salt levels, posing a risk of salt stress to seedlings. Bacillus spp. can alleviate salt stress and promote growth in various crops, supporting their use in saline environments. This study confirmed that Bacillus spp. enhanced cucumber seedling growth, especially B. velezensis, which showed the most significant growth-promoting and disease-preventing effects [27-29]. B. velezensis produces specific metabolic byproducts, including fungistatic compounds, spores, and peptide antibiotics, which promote growth, enhance nutrient uptake, and provide disease resistance [30]. Its strong biofilm-forming ability further supports plant growth and health by releasing beneficial metabolites and microbial communities. Genomic differences in B. velezensis contribute to its superior biological activity and ecological adaptability.
Fig. 4.
Effect of different Bacillus species on the microbial content of Fusarium in post-sedimentation substrates. Note: Different lowercase letters in the same column represent significant differences (P<0.05). CK represents the blank control, while T1, T2, and T3 represent Bacillus subtilis, Bacillus amyloliquefaciens, and Bacillus velezensis, respectively.
The findings of our study not only have strong implications for the development of seedling substrates but also apply to the formulation of related organic fertilizers, especially for the application of kitchen waste compost in field conditions. Currently, kitchen waste compost is widely used in paddy fields, where the presence of water dilutes the salt and grease content, thus greatly mitigating their adverse effects on rice growth [31]. However, there is a lack of research on the application of kitchen waste compost in dry fields, especially for vegetable crops. This gap is mainly due to the potentially strong inhibitory effects of salt in kitchen waste compost on vegetable growth. It is essential to clarify that using different composting processes for kitchen waste can lead to varying salinity levels, as evidenced by the germination index of compost produced through different methods [32, 33]. Additionally, kitchen waste is characterized by its complex composition [34]. Due to the diverse dietary habits in China, the composition of kitchen waste varies depending on cultural, regional, and economic factors. The differences in physicochemical properties are not limited to salinity but also include nutrient content and organic matter. Therefore, conducting research on kitchen waste composting faces numerous challenges. Nonetheless, the three Bacillus strains studied herein exhibited excellent performance in alleviating salt stress and promoting growth in cucumbers. Building upon these findings, incorporating Bacillus strains, particularly B. velezensis, into kitchen waste compost to produce bioorganic fertilizers may significantly promote the application of kitchen waste compost in vegetable production. However, it is worth noting that, despite achieving growth promotion, none of the three Bacillus strains in this study effectively absorbed Na+ and Cl- from the seedling substrate, resulting in no significant reduction in salt content compared to the control group. This remains a hidden risk in the field application of kitchen waste compost, as the accumulation of salt in the soil may lead to salinization, posing another significant challenge that requires further research for appropriate solutions.
Conclusions
In summary, Bacillus subtilis, Bacillus licheniformis, and Bacillus amyloliquefaciens all exhibit significant promotion of growth and disease prevention effects on cucumber seedlings in kitchen waste compost substrate. Among them, Bacillus amyloliquefaciens demonstrates the most optimal effects. It is recommended to further investigate solutions to the issue of residual salt ions from kitchen waste compost in the substrate or soil based on the results of our study.

