


Introduction
Drought, a significant abiotic stressor, poses a formidable challenge to various global regions. It disregards geographical boundaries and defies predictable patterns, manifesting across diverse environments. This unrelenting stress can profoundly impede plant production, compromise plant health, and undermine production quality. Its causal factors, including heightened temperatures, diminished light intensity, and insufficient rainfall, wield substantial influence. Urban population growth is one of the factors that cause climate change. Industrialization and irregular urbanization continue to have a negative impact on human life by triggering climate change [1]. Notably, Rashid et al. [2] emphasize its paramount impact as a pervasive environmental stressor, influencing every facet from cereal food security during production to post-harvest consumption.
For wheat, drought emerges as a pivotal determinant of poor productivity [3], exerting deleterious effects on crucial growth phases [4]. Ullah et al. [5] elucidate the hostile repercussions of drought at various growth junctures in wheat. At the tillering stage, it leads to diminished plant height and fewer tillers per unit area. Consequently, it contributes to reduced biomass, compromised spike formation, fewer grains per spike, and ultimately, diminished grain weight during the grain-filling stage. This cascading impact can precipitate substantial yield losses of up to 50% [6-8]. Plant structures are influenced by heavy metals like Bi, Cd, and Ni, which are difficult to decompose and bioaccumulate and can have toxic or carcinogenic effects [7]. High air pollution impacts plants due to genetic structure and environmental conditions, affecting their development, structure, and phenotypic characteristics. Drought's multifaceted assault on these critical growth stages underscores its significance as a yield-limiting factor in wheat cultivation.
The utilization of synthetic fertilizers plays a pivotal role in enhancing soil fertility, representing an integral facet of modern crop production practices. In particular, the application of inorganic nitrogen fertilizers stands out as a crucial strategy, providing crops with the necessary nitrogen for synthesizing nitrogenous biomolecules, as noted by Beatty et al. [9] and Bhanse et al. [10]. Nevertheless, it's important to recognize that synthetic nitrogen fertilizer is a finite resource, and its excessive usage carries adverse implications for both atmospheric conditions and the quality of surface- and groundwater environments. These implications, in turn, have repercussions for human health, a point emphasized by Vocciante et al. [11]. For instance, area serves as a readily accessible source of ammonia (NH3) nitrogen, along with ammonium ions (NH4+), serving plant needs. However, under surface broadcast applications, less than half of this urea is effectively utilized. A significant proportion is lost through volatilization and/ or denitrification, as highlighted by Ghorbani et al. [12]. This highlights the need for innovative approaches that simultaneously curtail the dependence on inorganic nitrogen fertilizers while adequately fulfilling the nitrogen requirements of crops. The development of such methods becomes imperative to strike a balance between agricultural productivity, the conservation of nonrenewable resources, and environmental integrity. Soil, the primary organic carbon source for terrestrial ecosystems, is significantly reduced, leading to decreased productivity, biological diversity damage, and ecosystem resilience [8]. Studies have shown that the use of domestic peat, bat guano, chicken and sheep manures, and vermicompost positively impacts certain plant growth.
Biological nitrogen fixation constitutes a specialized and intricate process organized by a distinct assemblage of prokaryotic microorganisms. These microorganisms possess a unique enzymatic process known as nitrogenase, which catalytically transforms atmospheric dinitrogen into ammonia (NH3), as elucidated by Zhang et al. [13]. The deliberate introduction of plant seeds to nitrogen-fixing bacteria, specifically those categorized as plant growth-promoting rhizobacteria (PGPR), presents a promising avenue for enhancing various parameters associated with plant growth and yield. This phenomenon is underpinned by a complex interplay of direct and indirect mechanisms organized by PGPR, as documented by Reyero-Saavedra et al. [14], Sarfraz et al. [15], Chieb and Gachomo, [16], and Ali et al. [17]. By enriching and fortifying the microbial populations residing within the root zone, PGPR exerts a profound influence on the intricate ecosystems of the root environment. This influence proves to be of paramount importance, especially in scenarios characterized by nutrient deficiency that could otherwise impede the attainment of optimal plant growth. The study suggests that regular application of vermicompost leachate, rich in nutrients and microbial activity, can improve salinity in salinized soils in arid and semi-arid areas, thereby enhancing soil and plant quality.
Concomitant with their nitrogen-fixing prowess, PGPR contributes to the synthesis of cytokinins, antibiotics, and hydrolytic enzymes. Collectively, these compounds play a pivotal role in fostering both root and shoot growth, as evidenced by the research of Bibi et al. [18]. This multifaceted role of PGPR highlights their significance as facilitators of growth-promoting processes in plants. The multifaceted influence of PGPR on plant growth is further manifested through the production of diverse phytohormones, with a particular emphasis on auxins, particularly indole-3- acetic acid (IAA) [19, 20]. These microorganisms also contribute enzymatic and non-enzymatic metabolites, such as proline, a pivotal nitrogen-derived antioxidant. Such metabolites play a pivotal role in neutralizing the deleterious effects of reactive oxygen species within plants [21]. Morphological and physiological transformations in the root architecture, orchestrated by PGPR, significantly enhance water and nutrient uptake [22, 23]. Research by Tanveer et al. [24] and others underscores the heightened germination rates, improved root development, increased crop yield, elevated leaf area, heightened chlorophyll content, and augmented nitrogen and protein levels witnessed in seeds inoculated with PGPR in comparison to their non-inoculated counterparts [25, 26]. Additionally, PGPR-mediated enhancements extend to bolstering drought tolerance in crops, as exemplified by studies like Dasila et al. [27]. The far-reaching impacts of PGPR find further validation in diverse crops such as wheat, rice, cotton [28, 24], canola, and maize [29], where seed inoculation culminates in amplified yields.
The process of seed inoculation involves the application of diverse bacterial strains before planting, where the pivotal requirement is the establishment of an optimal interaction with the seed. This interaction is fundamental for the survival of the microorganisms on the seed surface and subsequent colonization endeavors [30]. Among these strains, Azospirillum emerges as a diazotrophic bacterium with a substantial role in the rhizosphere of numerous plants. It demonstrates the capability to fix atmospheric dinitrogen and transform it into a form accessible to plants [31]. The practice of inoculating wheat seeds with Azospirillum spp. has found widespread application in augmenting crop yields across diverse soil compositions [26].
However, the outcomes of PGPR inoculation haven't consistently yielded success, and the factors governing growth responses remain incompletely elucidated. The intricate interplay between different Azospirillum spp. strains and wheat crops have been reported [27, 26]. The establishment of Azospirillum spp. in plant roots comprises two distinct phases, the adsorption and anchoring phases, facilitated by surface polysaccharides and lectins [32].
The present study endeavors to investigate the influence of sole and co-inoculation with A. lipoferum and A. fabrum, two distinct biological nitrogen-fixing bacteria, on the growth and physiological attributes of wheat crops.
Experimental
The research was conducted during 2022-23 within the wirehouse facilities of the Department of Agronomy at the Islamia University of Bahawalpur, Pakistan. The experimental setup encompassed pots arranged in a random complete block design, consisting of four primary treatments, each replicated three times. These treatments were designated as follows: T0 = control without inoculation, T1 = involving the inoculation of Azospirillum lipoferum, T2 = involving the inoculation of Agrobacterium fabrum, and T3 = co-inoculation of both A. lipoferum and A. fabrum.
Soil Analysis
A detailed examination of the soil's physicochemical attributes revealed a composition characterized by 15% sand, 15% silt, and 70% clay, alongside 0.79% organic matter, 0.37 mg kg−1 dry soil nitrogen, 5.1 mg kg−1 dry soil phosphorus, 119 mg kg−1 dry soil potassium, and a soil pH of 7.1.
Pot Experiment
To augment the experimental conditions, the recommended dosage of N-P-K fertilizer at a rate of 150-115-62 kg ha−1 was employed in the pots. The two strains of PGPR employed, specifically A. lipoferum and A. fabrum, were sourced from the Ayub Agricultural Research Institute in Faisalabad, Pakistan. Similarly, the wheat seeds utilized in the study were procured from the Regional Agriculture Research Institute in Bahawalpur, Pakistan.
Seed Inoculation
To ensure optimal conditions, the surface of the wheat seeds was subjected to sterilization. This involved a sequential treatment of the seeds with 70% ethanol for 2 minutes, followed by a 30-minute exposure to 5% sodium hypochlorite. Subsequently, the wheat seeds were inoculated with A. lipoferum and A. fabrum at a concentration of 10 × 108 colony-forming units and harvested at the exponential growth phase. The inoculation process was standardized to an application of 150 cm3 per 50 kg of wheat seeds, with an equivalent volume employed for co-inoculation. In their study, Fukami et al. [32] delineated the procedure for inoculating Plant Growth-Promoting Rhizobacteria (PGPR) onto wheat seeds and subsequently transplanting them into pots. The pots, measuring 25×25 cm in dimensions, were loaded with 9 kg of soil, and a total of nine seeds were meticulously sown within each pot. This sowing process was executed on the 15th of November, 2022. Notably, the experimental setup involved the cultivation and maintenance of three plants within each of these pots.
Growth Parameters
The assessment of various crop growth and yield-related parameters was carried out to gauge the performance of the cultivated wheat. These parameters encompass plant height, spike length, the number of spikelets per spike, the number of grains per spike, 1000-grain weight, and grain yield per plant. The measurement process spanned from the initial stages of cultivation to the point of wheat maturity and final harvest. These evaluations adhered to established protocols and standards. For a comprehensive understanding of growth dynamics, critical indices were computed. The rate of increase in total dry weight per unit area (CGR), the rate of increase in total dry weight per individual plant (RGR), and the leaf area index (LAI) were meticulously quantified. These assessments followed the methodologies prescribed by Gardner et al. [33].
Physiological Parameters
Transpiration rate, a pivotal physiological parameter, was quantified using an infrared gas analyzer (LCA-4, ADC, UK), employing the procedure outlined by Long and Bernacchi [34]. Similarly, the relative water content (RWC) was measured utilizing the formula introduced by Barrs and Weatherley [35], factoring in the fresh weight, dry weight, and total fresh weight of the wheat. Furthermore, the content of epicuticular wax on the leaf surface was determined based on leaf area, employing the approach recommended by Silva Fernandes et al. [36]. The assessment of relative chlorophyll content was facilitated through the employment of a Soil-Plant Analyses Development (SPAD) device (Minolta Camera Co., Japan). Additionally, the quantification of proline content was carried out through spectrophotometry, using the ninhydrin method as outlined by Bates et al. [37].
PGPR Analysis for Production of Auxin
To ascertain the production of auxin-inducing rhizobacteria containing L-tryptophan, a colorimeter-based methodology was employed. The cultivation of Plant Growth-Promoting Rhizobacteria (PGPR) occurred in L-broth L-tryptophan (500) for three days under conditions of 150 rpm and 30°C. A non-inoculated control was concurrently maintained for comparative purposes. After bacterial culture, centrifugation was carried out, and the resulting supernatant (1 mL) was combined with Salkowski's reagent (2 mL). The quantification of Auxin production was facilitated by establishing a standard curve using authentic Auxin. Furthermore, the supernatants from the same strains underwent analysis through Ultra-Performance Liquid Chromatography (UPLC). Acidification of the supernatant to a pH of 2.5 with 1N HCL was executed, followed by triple extraction with an equivalent volume of ethyl acetate. To assess the quantity of Auxin produced.
Results
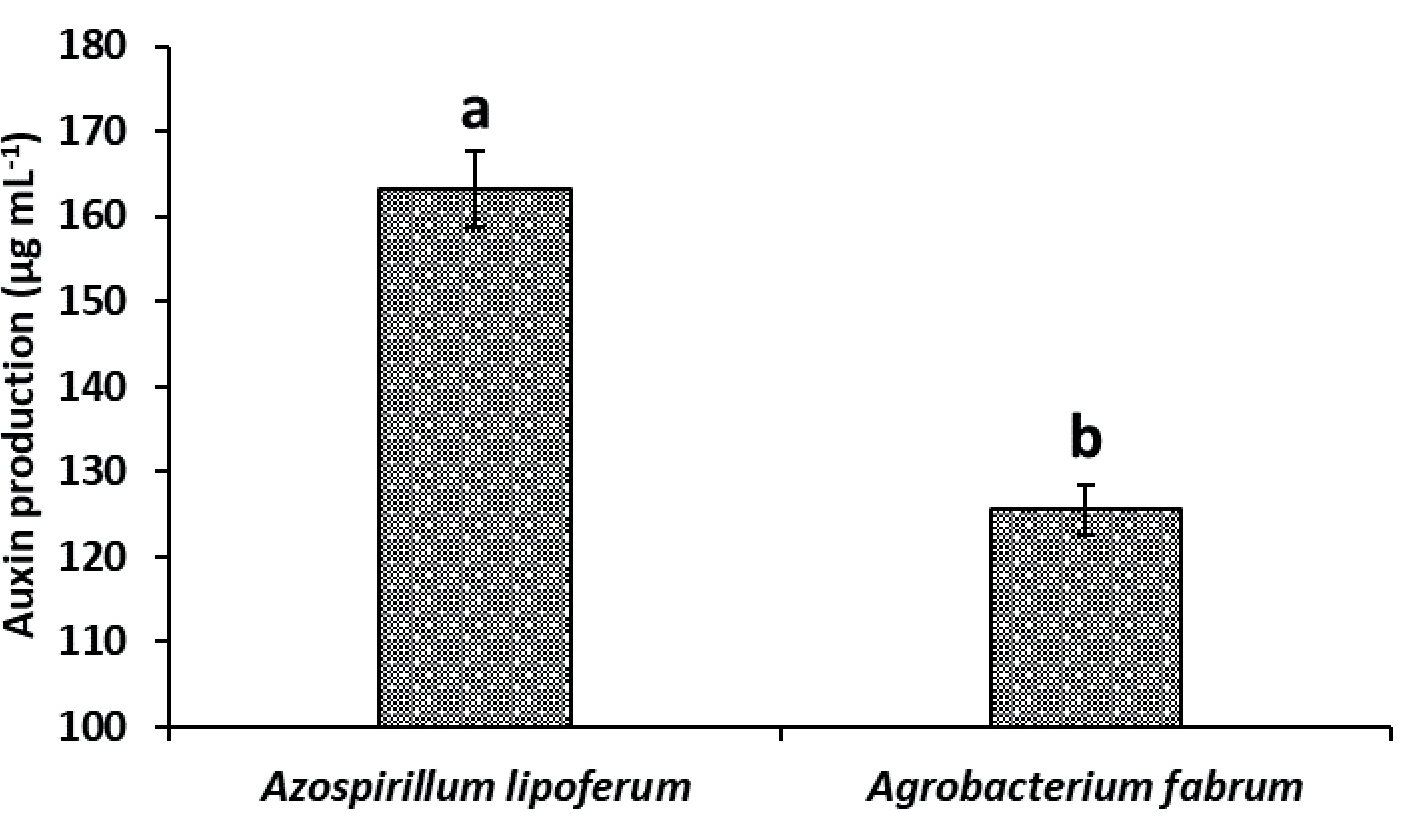
Auxin production by different PGPR strains is shown in Fig. 1. The result of our experiment shows that maximum Auxin (163.24 µg mol-1) is produced by the PGPR strain Azosprillium lipoferum and (125.53 µg mol-1) was produced by Agrobacterium fabrum. Table 1 represents the different levels of Indolic compounds. The highest level of ILA (14.2 µg mol-1) was released by strain Azosprillium lipoferum, followed by strain Agrobactrum fabarum (14 µg mol-1). A maximum level of ICA was noticed in strain Azosprillium lipoferum (0.8 µg mol-1) and (0.3 µg mol-1) in strain Agrobacterium fabarum. The highest level of IAA (5.5 µg mol-1) was observed by strain Azosprillium lipoferum, followed by strain Agrobacterium fabarum (3.3 µg mol-1).
Table 2.
Effect of seed inoculation of A. lipoferum and A. fabarum on growth and physiological parameters of wheat.
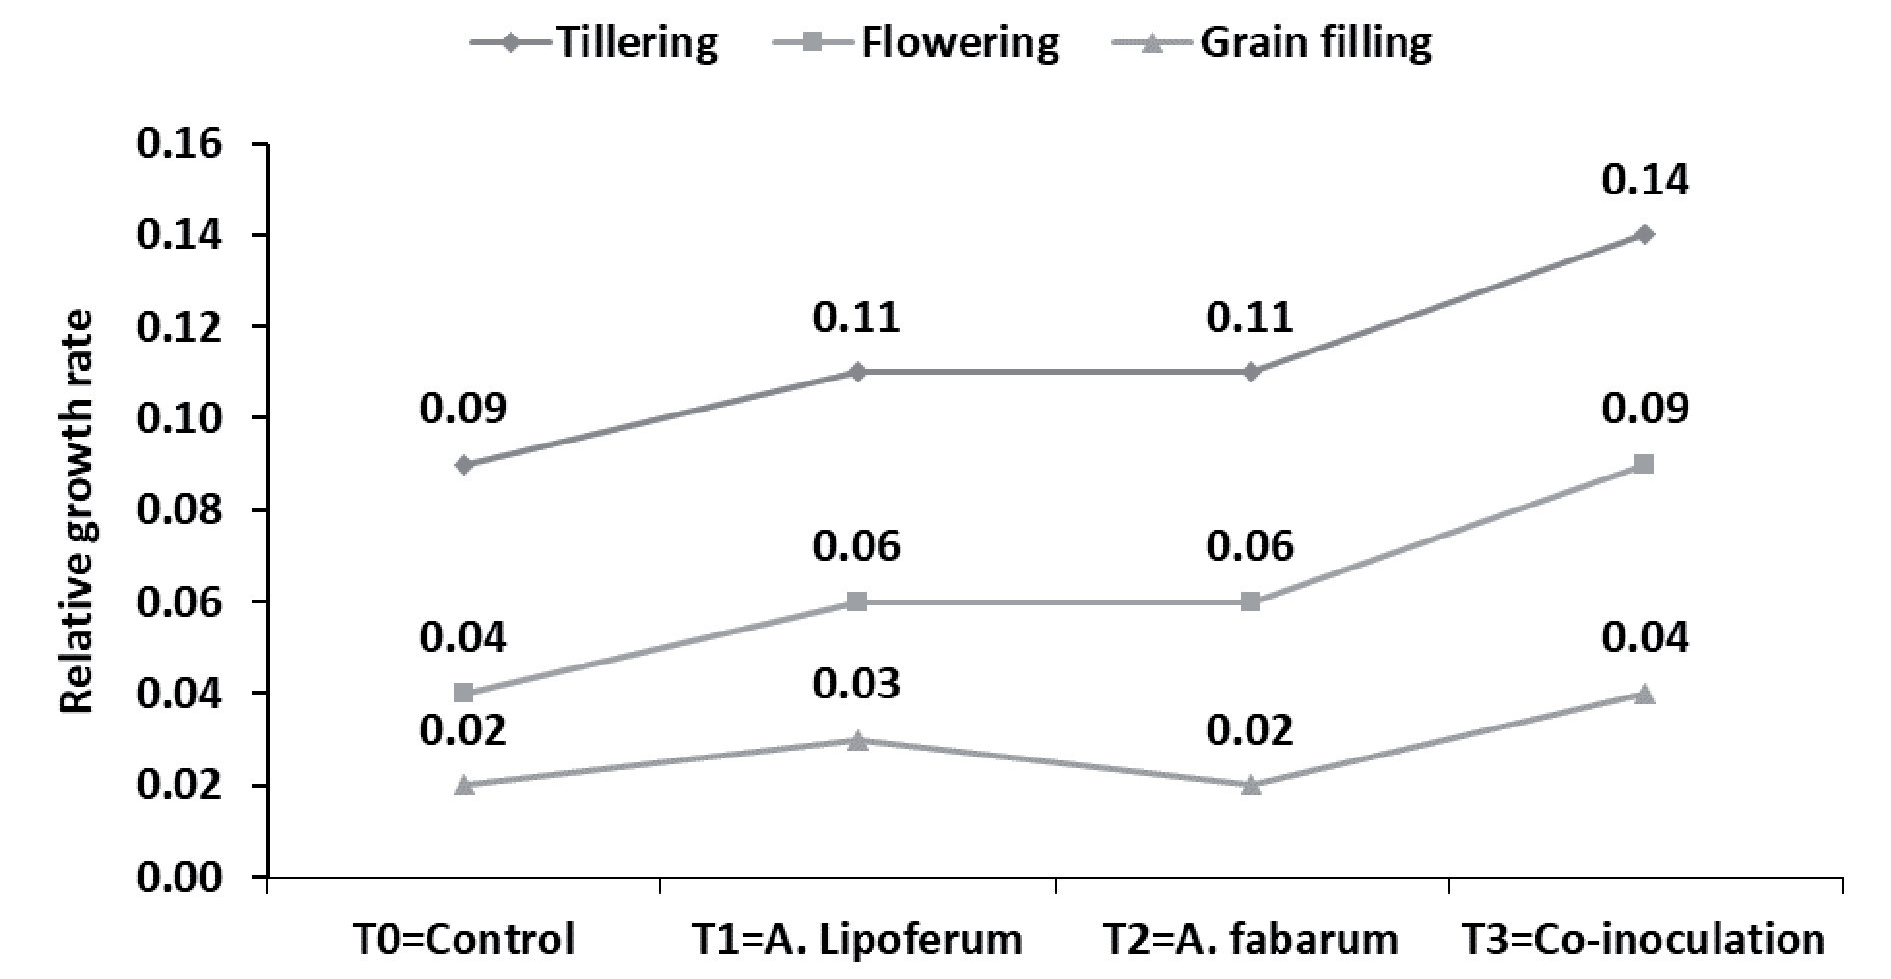
Table 3.
Effect of seed inoculation of A. lipoferum and A. fabarum on growth and physiological parameters of wheat.
| Treatments | CGR at Tillering | CGR at Flowering |
|---|---|---|
| Control | 1.75 b | 7.31 c |
| 1.95 b | 9.52 b | |
| A. fabrum | 1.95 b | 9.49 b |
| A. lipoferum + A. fabrum | 2.21 a | 10.61 a |
| Single PGPR vs control | N.S | * |
| Single PGPR vs co-inoculation | N.S | * |
The study revealed the modest importance of inoculation on plant height concerning the factors connected with plant morphology and yield characteristics. Significantly, treatments T1 and T2 demonstrated a higher level of plant height in comparison to the non-inoculated control, referred to as T0. It is noticed that treatment T3 resulted in the greatest plant height; yet, there was no statistically significant difference in plant height between treatments T1, T2, and T3, as shown by the data presented in Table 2. This finding deserves further consideration. Characteristics such as the length of spikes, the number of spikelets per spike, the number of grains per spike, and the weight of 1000 grains exhibited comparable reactions to the treatments, including inoculation. The treatment T3 exhibited the highest significant results, followed closely by T1 and T2. Significantly, the statistical analysis revealed that there was no significant difference between the results of T1 and T2, suggesting that they had a similar influence. In contrast, the treatment T0 had the lowest values for these variables. The observed difference between sole and co-inoculation strategies was statistically significant for all the characteristics. Treatment T3 produced the most grains per plant, (1.723 g). After that, treatments T1 and T2 yielded (1.531 g) and (1.516 g), respectively, which show statistically significant differences. T0, which did not inoculate, produced the least grain per plant (1.261 g). These findings show that inoculation improves plant growth and production attributes.
The inoculation with the two Plant Growth-Promoting Rhizobacteria did not affect the Crop Growth Rate (CGR) during tillering. However, the co-inoculated therapy had little statistical significance compared to the other treatments (Table 3). At the flowering stage, the inoculated (T1 and T2) and co-inoculated (T3) treatments had CGR values of 37% and 52% greater than the control (T0) treatment. Comprehensive research shows that treatment T3 had the highest CGR values. The tillering and flowering stages had CGR levels of 2.21 and 10.61 g m−2 day−1, respectively. Following closely were T1 and T2. Compared to treatment T0, the tillering and flowering stages had the lowest CGR values of 1.75 and 7.31 g m−2 day−1, respectively. This complete examination shows that the co-inoculation strategy (T3) yields the greatest CGR values throughout both development phases, suggesting that combined PGPR treatment may boost crop growth.
In Fig. 2, it is shown that the tillering stage had the greatest relative growth rate (RGR) across all treatments, followed by the flowering stage. Conversely, the grain-filling stage displayed the lowest RGR. The relative growth rate (RGR) of wheat was shown to be strongly influenced by the inoculation of plant growth-promoting rhizobacteria (PGPR). Furthermore, the RGR of treatment T3 continuously exhibited considerably higher values compared to treatment T0. Similarly, the RGR of treatments T1 and T2 also demonstrated significantly higher values compared to treatment T0.
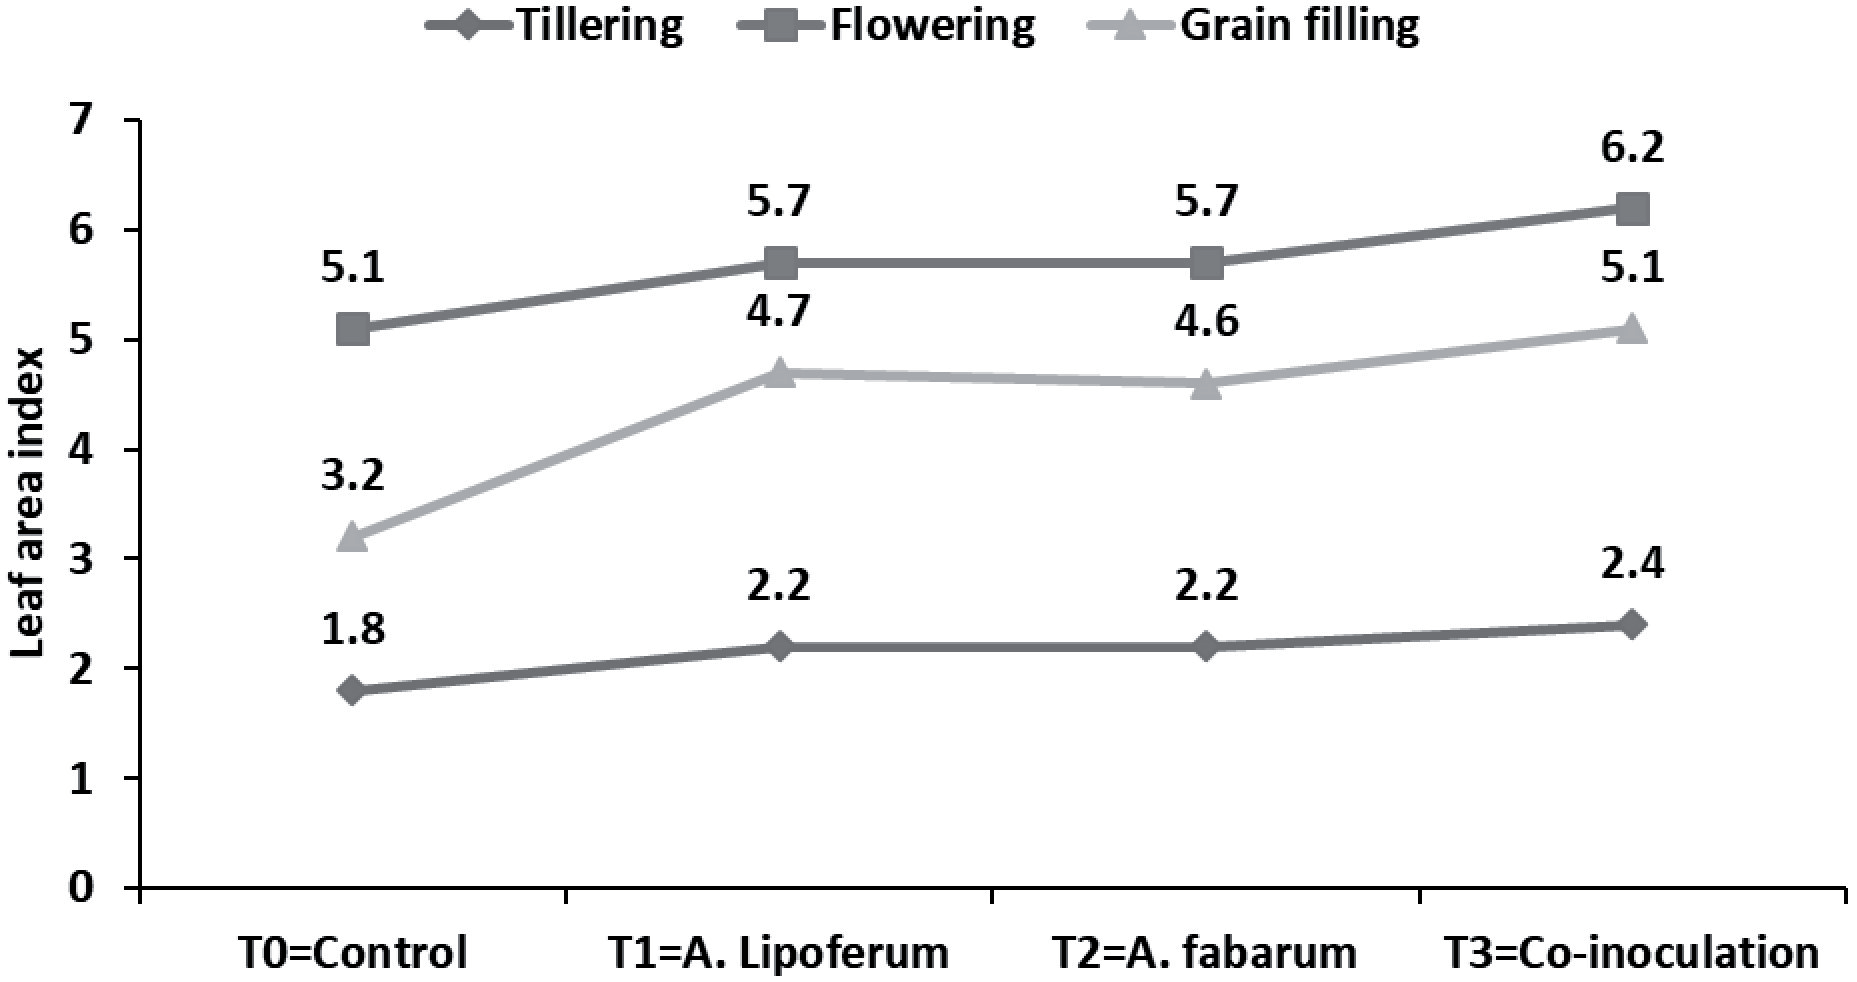
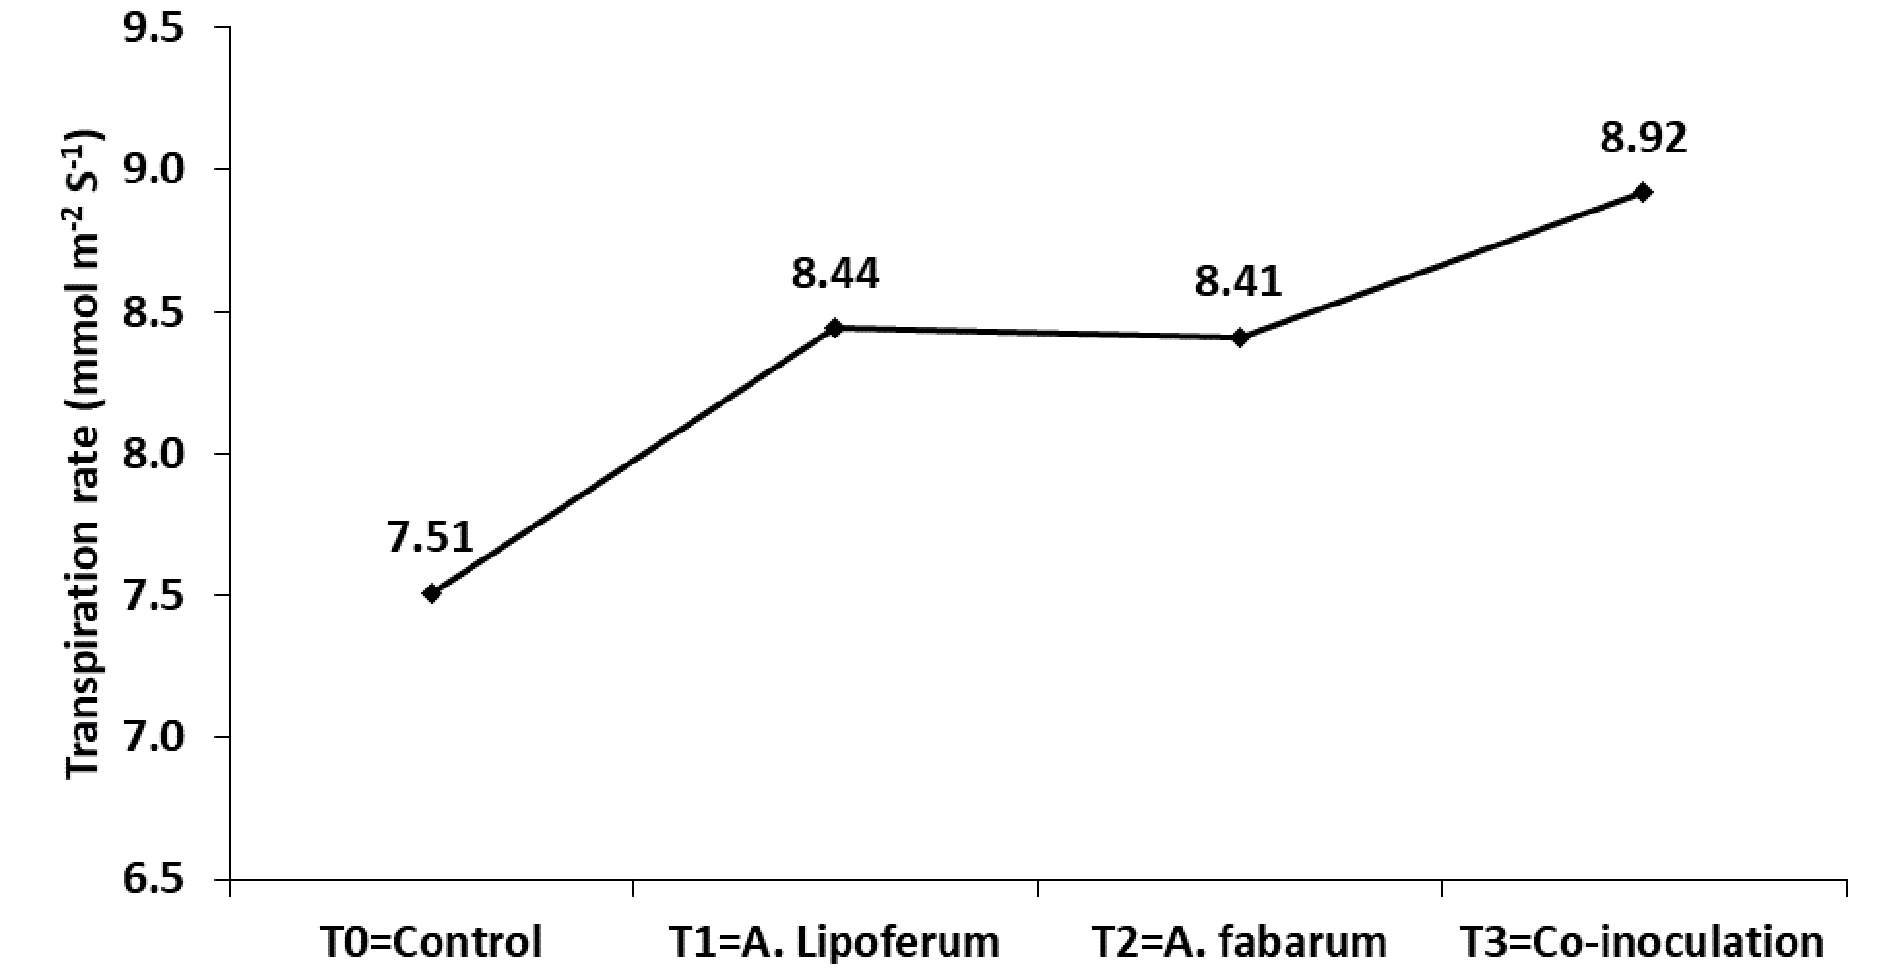
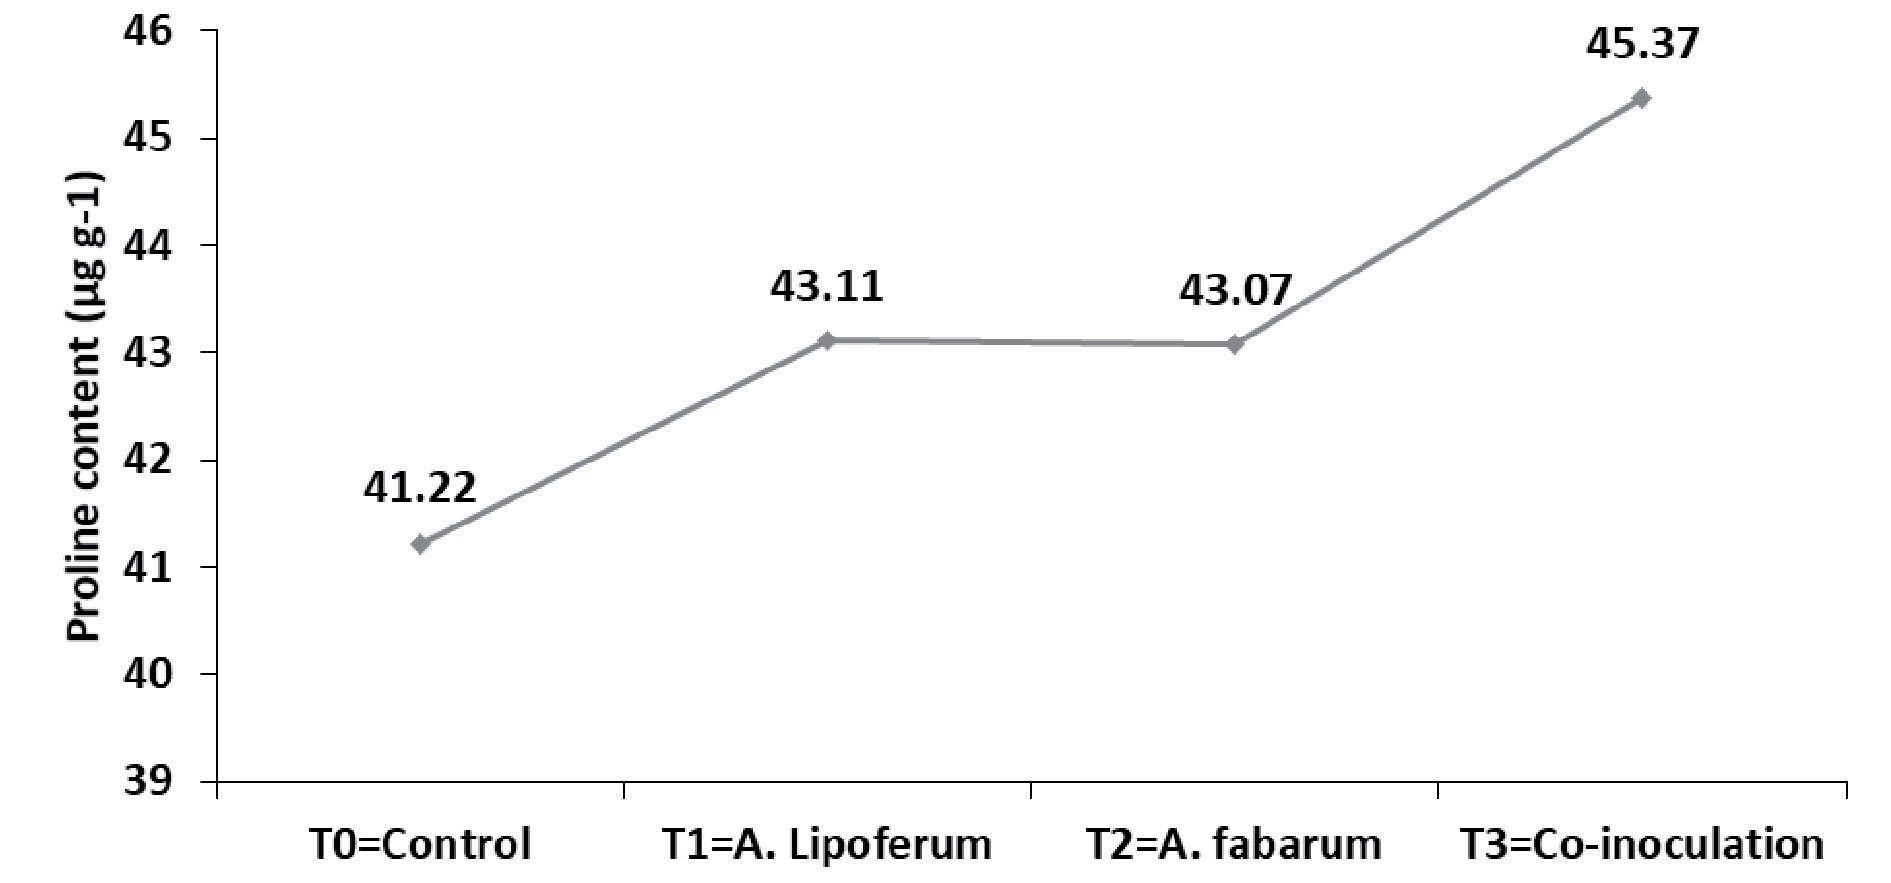
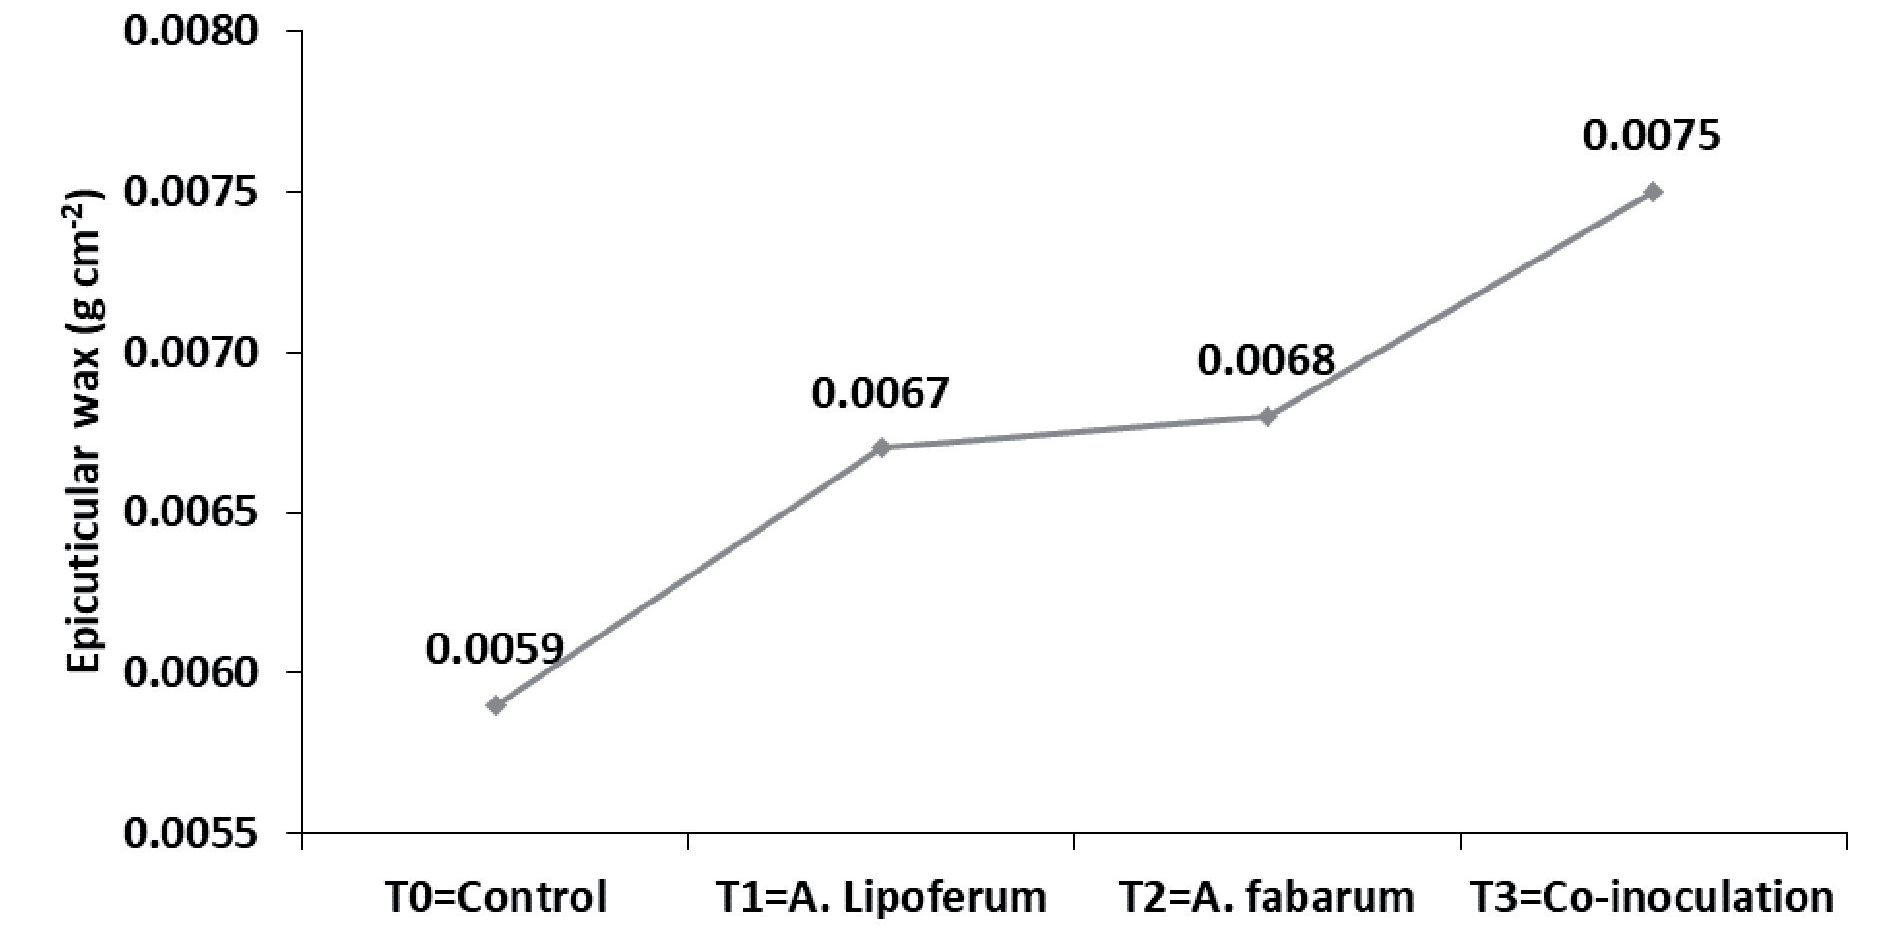
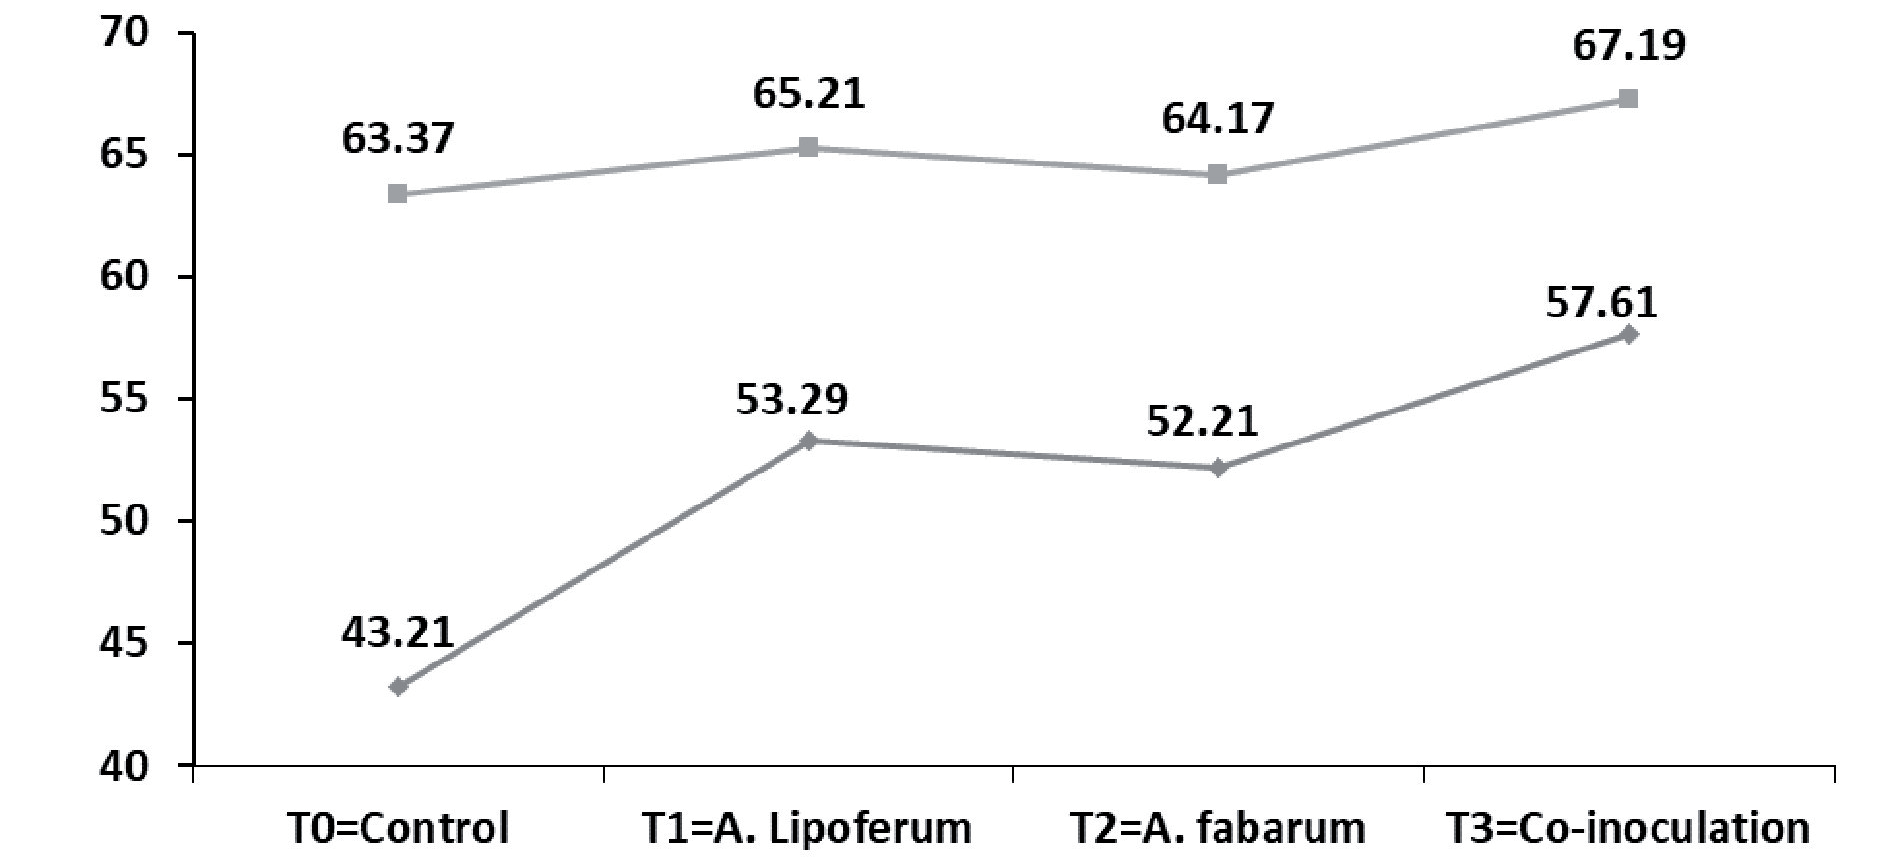
The Leaf Area Index (LAI) of Treatment (T3) exhibited the greatest value, which was shown to be statistically distinct from the LAI values of the other treatments (Fig. 3). Following T3, T1 and T2 had comparable LAI values, which were considerably greater than the LAI value of T0. The inoculation of PGPR had significant effects on leaf transpiration rate (Fig. 4), proline content (Fig. 5), and epicuticular wax content (Fig. 6). Among the treatments, T3 exhibited the greatest values for these variables, followed by T1 and T2, which had comparable values. However, T0 had the lowest values for all variables. Nevertheless, the transpiration rate (Fig. 4) exhibited no statistically significant difference between the treatments where the solo inoculation was applied and those where co-inoculation was implemented. The application of PGPR had a considerable impact on the chlorophyll content of wheat (Fig. 7). The highest levels of chlorophyll (54%) were seen in treatment T3, followed by treatments T1 and T2. There was no statistically significant difference seen in the chlorophyll content between T1 and T2 treatments. However, the treatment labeled as T0 exhibited the lowest chlorophyll content, measuring 44%. Additionally, the root water content (RWC) of wheat was influenced by the presence of plant growth-promoting rhizobacteria (Fig. 7). Similar to the results observed for the other variables, the highest RWC (73%) was observed in the co-inoculated treatment (T3), while the lowest RWC (61%) was observed in the control treatment (T0). The sole inoculation treatments (T1 and T2) fell between these extremes and were not statistically different from each other.
Discussion
The assessment of Plant Growth-Promoting Rhizobacteria (PGPRs) through the lens of auxin production yields considerable advantages. Through the application of colorimetric analysis, all bacterial strains cultivated on an L-tryptophan-adjusted medium exhibited proficient synthesis of indole-3- acetic acid (IAA), a crucial auxin. Among the various auxins, including indole-3-lactic acid (ILA), indole- 3-carboxylic acid (ICA), and IAA, it has been well documented that these play pivotal roles in plant growth regulation. The emergence of diverse indolic compounds points to distinct pathways governing IAA synthesis. Notably, prior research by Belimov et al. [38] has underscored the existence of indolic compounds in the growth of bacterial strains like P. oryzihabitans Ep4, Achromobacter xylosoxidans Cm4, and Variovorax paradoxus 5C-2. Furthermore, the work of Goswami et al. [39] has revealed that within bacterial cultures, IAA, indole-3-butyric acid (IBA), and indole-3-propionic acid (IPA) are among the compounds produced. In the context of the current study, a crucial selection criterion for identifying PGPRs revolves around the assessment of auxin production by bacterial strains. This criterion serves as a fundamental cornerstone for the meticulous selection process of PGPRs in the scope of this investigation.
The use of Plant Growth-Promoting Rhizobacteria (PGPR) resulted in a significant increase in both spike length and spikelet count per spike. The data reported in Table 2 clearly illustrates the observable improvements. This finding is consistent with the findings published by Hyder et al. [25]. Both of these factors have a role in determining the overall economic output of the crop. In the case of several crops, around 80% of PGPR generates phytohormones as secondary metabolites inside the rhizosphere [40, 17]. These phytohormones have a direct positive impact on both plant development and the number of spikelets per spike. Furthermore, it was observed that the number of grains per spike was significantly larger in the inoculated group compared to the non-inoculated group, which aligns with the results published by Ullah et al. [41]. In their study, Ullah et al. [41] also found a greater number of grains per spike in wheat plants that were subjected to PGPR inoculation. In addition, it has been shown that PGPR (plant growth-promoting rhizobacteria) are capable of synthesizing a range of plant growth hormones, including indole-3- acetic acid (IAA), which has been shown to enhance grain weight [42, 43].
Grain yield is a significant factor of interest for researchers in the field of agro-environmental studies. In comparison to the control group T0, the findings of this study indicate a notable rise of around 36% in grain production per plant for T3. Additionally, T1 and T2 exhibited an increase of approximately 25% in grain yield. This phenomenon may likely be attributed to the influence of PGRP on several other variables related to nutrient availability and absorption, including but not limited to RGR, transpiration rates, and LAI [41]. According to Sharafzadeh [30], it has been shown that PGPR may induce morph physiological alterations in the root, leading to enhanced water and nutrient absorption, eventually resulting in increased grain production. Plant growth-promoting rhizobacteria (PGPR) have been shown to boost plant development via many mechanisms. One such mechanism is the facilitation of nutrient mobilization and absorption from the soil, leading to increased nutrient availability for the plants. Additionally, PGPRs are known to produce growth regulators, which may further stimulate plant growth. Furthermore, these bacteria have been seen to improve the structure of the soil, therefore creating a more favorable environment for plant growth [15]. Previous research has shown that the application of plant growth-promoting rhizobacteria (PGPR) has yielded beneficial outcomes on crop growth and development. These good benefits may be attributed to enhanced nutrient absorption from the soil and reduced water stress, as reported by Ditta and Ullah [44, 45]. Additionally, the presence of PGPR has been found to mitigate the detrimental impact of phytopathogenic organisms while also improving antibiosis and competitive exclusion, as highlighted by Ibrahim and El-Sawah, [46].
In the current study, significant differences were observed in the crop growth rates (CGRs) during the tillering and flowering stages (Table 3). Specifically, there was a 5.37% increase in CGR for sole inoculations (T1 and T2) compared to the control group (T0) at the tillering stage and a 33.47% increase at the flowering stage. Additionally, co-inoculation (T3) resulted in a 9.16% higher CGR at the tillering stage and a 14.96% higher CGR at the flowering stage, in comparison to T1 and T2 (Table 3). At all phases of development, the treatment T0 consistently exhibited the lowest relative growth rate (RGR). Conversely, the maximum RGR was consistently recorded during the tillering stage, surpassing RGR at the flowering and grain-filling stages by about 55% and 86%, respectively (Fig. 2). During the tillering stage, the relative growth rate (RGR) exhibited a 55% increase for treatments T1 and T2, while treatment T3 showed a higher increase of 83% compared to the control treatment (T0). The growth regulator status of wheat, which is mostly influenced by environmental pressures, is likely to have been improved or maintained with the assistance of PGPR [47].
A significant difference was seen in the Leaf Area Index (LAI) between wheat plants subjected to inoculation and those in the control group. Furthermore, the co-inoculation treatment exhibited the greatest LAI, as shown in Fig. 3. In addition, the Leaf Area Index (LAI) exhibited a progressive rise from the tillering stage to its peak values during the flowering stage, afterward undergoing a gradual fall as the crop advanced in age. According to Ahmad et al. [48], the leaves of the plant underwent senescence. Indeed, many variables that were examined, including CGR and LAI, exhibited their peak values at the flowering stage. The flag leaf plays a crucial role in the transportation of carbohydrates to the grain. Consequently, the occurrence of physical-environmental challenges, such as water or nutrient deprivation, during the flowering stage may have a significant impact on crop development and ultimately influence the final grain yields of the crop. High air pollution impacts plants due to genetic structure and environmental conditions, affecting their development, structure, and phenotypic characteristics [49].
The experimental treatment T3 exhibited a transpiration rate that was 14% greater than the control treatment T0. This phenomenon may likely be attributed to the fact that the application of PGPR increased the density of wheat roots, leading to higher water absorption. Additionally, previous research has shown that PGPR plays a role in improving the hydraulic properties of roots, hence contributing to the maintenance of plant water relations and ultimately enhancing the rate of transpiration [27]. In addition, it has been observed that wheat plants have the ability to accumulate osmolytes, which can increase proline content [50]. Furthermore, it has been suggested that plant growth-promoting rhizobacteria (PGPR) may play a role in enhancing proline content (Fig. 5), potentially by improving the synthesis of abscisic acid, which is responsible for regulating the expression of the proline synthesis gene P5CS [51, 52].
Furthermore, the levels of chlorophyll content and relative water content (RWC) were found to be significantly greater in the infected treatments as compared to the control group (Fig. 7). According to Shrestha et al. [53], elevated chlorophyll content has the potential to enhance the photosynthetic rate. Additionally, the presence of plant growth-promoting rhizobacteria (PGPR) aids in the improvement of leaf area index (LAI) and stomatal conductance, hence facilitating the enhancement of relative water content [54]. It has been shown that leaves of greater size have higher levels of chlorophyll concentration.
Conclusions
In the present study, the use of A. lipoferum and A. fabrum, either alone or in combination, has been shown to have notable and advantageous impacts on the growth and productivity of wheat farmed under controlled conditions. Significant improvements were noted in various aspects, including growth dynamics (such as Leaf Area Index and plant height), physiological indicators (such as chlorophyll and proline contents), water-related attributes (such as Relative Water Content and transpiration rate), and yield-contributing factors (such as grain weight and yield). Significantly, co-inoculation consistently resulted in the highest results within this framework. Based on these findings, it is clear that the application of A. lipoferum and A. fabrum as inoculants for wheat seeds, either individually or in combination, presents a promising approach to augment the growth, productivity, and overall characteristics of wheat crops when compared to situations where no inoculation is performed. However, more research endeavors must be undertaken to expand upon and validate these findings under field conditions.

